研究论文

饲粮非植酸磷水平对14日龄仔鹅肠道组织形态、食糜酶活性及菌群结构的影响

  • 黄春慧 ,
  • 李宁 ,
  • 胥蕾 , * ,
  • 正旭城 ,
  • 杨海明 ,
  • 王志跃
展开
  • 扬州大学动物科学与技术学院,扬州 225009
*胥 蕾,副教授,硕士生导师,E-mail:

黄春慧(1998—),女,江苏盐城人,硕士研究生,研究方向为家禽生产与营养。E-mail:

Copy editor: 陈鑫

收稿日期: 2023-09-22

  网络出版日期: 2024-03-13

基金资助

财政部和农业农村部国家现代农业产业技术体系资助(CARS-42-11)

江苏省现代农业(水禽)产业技术体系建设专项资金资助(JATS[2022]496)

Effects of Dietary Non-Phytic Phosphorus Levels on Intestinal Morphology, Chyme Enzyme Activities and Microbial Structure of 14-Day-Old Goslings

  • HUANG Chunhui ,
  • LI Ning ,
  • XU Lei , * ,
  • ZHENG Xucheng ,
  • YANG Haiming ,
  • WANG Zhiyue
Expand
  • College of Animal Science and Technology, Yangzhou University, Yangzhou 225009, China
*associate professor, E-mail:

Received date: 2023-09-22

  Online published: 2024-03-13

摘要

本试验旨在通过研究饲粮非植酸磷(NPP)水平对14日龄仔鹅肠道生长、肠道重要酶活性、肠道组织形态以及空肠菌群结构的影响,探究NPP水平影响仔鹅生长性能的作用机制。选取216只1日龄的江南白鹅公鹅,随机分为3组,每组6个重复,每个重复12只。3组饲粮NPP水平依次为0.08%(低磷组,LP组)、0.38%(对照组,CP组)、0.80%(高磷组,HP组)。试验期14 d。结果表明:1)LP组十二指肠、空肠和回肠的绝对长度、绝对重量显著低于CP组和HP组(P<0.05),CP组与HP组的肠道绝对长度没有显著差异(P>0.05);而LP组肠道相对长度均显著高于CP组和HP组(P<0.05),CP组肠道相对长度显著高于HP组(P<0.05);LP组和CP组肠道相对重量没有显著差异(P>0.05),LP组和CP组空肠和回肠的相对重量显著高于HP组(P<0.05)。2)LP组十二指肠黏膜碱性磷酸酶活性显著低于HP组(P<0.05);LP组空肠Na+-K+ATP酶的活性显著低于CP组和HP组(P<0.05),CP组和HP组之间Na+-K+ATP酶活性没有显著差异(P>0.05)。3)不同组间各肠段的绒毛高度、隐窝深度、肌层厚度无显著差异(P>0.05)。4)LP组空肠代尔夫特菌属(Delftia)、苍白杆菌属(Ochrobactrum)、不动杆菌属(Acinetobacter)和黄杆菌属(Flavobacterium)的相对丰度显著高于CP组和HP组(P<0.05);TM7和厚壁菌门(Firmicutes)的相对丰度显著高于CP组和HP组(P<0.05);在属水平和门水平下,CP组和HP组之间的菌群相对丰度没有显著差异(P>0.05)。综上所述,仔鹅饲粮NPP水平过低可代偿性地增加肠道相对长度,但其造成的肠道功能性酶活性下降、空肠菌群结构失衡可能是饲粮低磷导致仔鹅生长性能下降的重要原因;同时鹅可耐受高达0.80%的NPP且对仔鹅早期肠道发育、空肠菌群结构无负面影响。

关键词: ; 非植酸磷; 肠道; 微生物

本文引用格式

黄春慧 , 李宁 , 胥蕾 , 正旭城 , 杨海明 , 王志跃 . 饲粮非植酸磷水平对14日龄仔鹅肠道组织形态、食糜酶活性及菌群结构的影响[J]. 动物营养学报, 2024 , 36(3) : 1674 -1684 . DOI: 10.12418/CJAN2024.147

Abstract

This study was conducted to investigate the effects of dietary non-phytate phosphorus (NPP) levels on the intestinal growth, activities of important intestinal enzymes, intestinal morphology and jejunal microbial structure of 14-day-old goslings, and to explore the mechanism of NPP levels on the growth performance of goslings. A total of 216 one-day-old male Jiangnan White geese were randomly divided into three groups, with six replicates in each group and 12 geese in each replicate. The dietary NPP levels of the three groups were 0.08% (low phosphorus group, LP group), 0.38% (control group, CP group) and 0.80% (high phosphorus group, HP group). The experiment lasted for 14 days. The results showed as follows: 1) the absolute length and weight of duodenum, jejunum and ileum in LP group were significantly lower than those in CP group and HP group (P<0.05). There was no significant difference in the absolute length of intestine between CP group and HP group (P>0.05). The relative length of intestine in LP group was significantly higher than that in CP group and HP group (P<0.05), and the relative length of intestine in CP group was significantly higher than that in HP group (P<0.05). There was no significant difference in the relative weight of the intestine between LP and CP groups (P>0.05). The relative weight of jejunum and ileum in LP and CP groups was significantly higher than that in HP group (P<0.05). 2) The alkaline phosphatase activity of the duodenal mucosa was lower in LP group than in HP group (P<0.05); the Na+-K+ ATPase activity was lower in LP group than in the CP group and HP group (P<0.05), there was no significant difference in Na+-K+ ATPase activity between the CP group and the HP group (P>0.05).3) No difference was observed in the villus length, crypt depth, and muscle layer thickness of each intestinal segment between groups (P>0.05). 4) The relative abundances of Delftia, Ochrobactrum, Acinetobacter and Flavobacterium were significantly higher in LP group than in the CP group and HP group (P<0.05), the relative abundances of TM7 and Firmicutes were significantly higher in LP group than in the CP group and HP group (P<0.05), there was no significant difference in microbiota relative abundance between the CP group and the HP group at the genus and phylum levels (P>0.05). In conclusion, goslings fed low dietary NPP level can compensatory increase in the relative length of the intestine, but the consequence of lower intestinal functional enzymes’ activity and imbalance of jejunal microbial structure may be important reasons for the decline of growth performance; at the same time, geese can tolerate NPP up to 0.80% and has no negative impact on the early intestinal development and jejunal microbial structure of geese.

磷是动物体内的必需矿物元素,参与动物机体的生长发育及生命活动,维持了动物机体正常的生理功能。Heyer等[1]研究发现,磷具有支持免疫系统和维持肠道组织结构的功能。有研究表明,饲料中含有适宜的磷可以显著提高鱼类肠道长度和重量[2-3]。黄学琴[4]认为降低肉鸭饲粮的营养和非植酸磷(NPP)水平,可降低肉鸭肠道的绒毛长度和隐窝深度。根据以上报道可知,NPP对于动物肠道生长具有重要作用。家禽饲粮中的磷大多以植酸磷的形式存在[5],但家禽体内不产生植酸酶,对植酸磷的利用率较低[6],因此应在家禽饲粮中添加NPP。微生物的各种代谢过程都需要磷的参与[7],家禽肠道内存在大量的微生物,影响家禽的健康及生产性能[8]。肠道微生物在家禽营养吸收、饲料消化能力和免疫反应等方面起到了十分重要的作用[9]。Mann等[10]研究发现,饲粮中钙、磷含量增加,可促进断奶仔猪胃内乳酸杆菌相对丰度增加14.9%。Borda-Molina等[11]研究发现,在饲粮中添加钙、磷和植酸酶后,显著影响肉鸡肠道中微生物的定植。有研究报道,不同的钙、磷添加量对肉鸡肠道内的菌群构成和丰度产生影响[12]。目前,饲粮NPP水平与仔鹅肠道微生物间的相互作用研究甚少。本团队的前期研究表明,饲粮NPP水平显著影响仔鹅生长性能,低磷组14日龄仔鹅体重、平均日增重和平均日采食量都低于对照组和高磷组[13],但其作用机制尚未明确。在此基础上,本研究拟从仔鹅肠道形态、食糜酶活性及菌群结构等方面探究饲粮NPP水平对14日龄江南白鹅仔鹅消化功能的影响及饲粮NPP水平影响仔鹅生长性能的作用机制。

1 材料与方法

1.1 试验设计

试验采用单因素试验设计。本试验选用216只1日龄体重相近、身体健康的江南白鹅公鹅作为试验动物。试验全期试验鹅自由采食、饮水,自然光照并按常规免疫程序进行免疫,保持圈舍卫生及通风良好。将试验动物分为3组,每组6个重复,每个重复12只鹅。3个组的饲粮NPP水平分别为0.08%(低磷组,LP组)、0.38%(对照组,CP组)、0.78%(高磷组,HP组)。试验期为14 d。

1.2 试验饲粮

采用玉米-豆粕型饲粮作为基础饲粮,饲粮组成参照Li等[10]。主要原料包括:玉米、豆粕、小麦麸、稻壳等。LP组、CP组和HP组饲粮营养水平:代谢能均为11.24 MJ/kg;粗蛋白质水平分别为18.29%、18.37%和18.44%;粗纤维水平均为4.27%;钙水平分别为0.76%、0.78%和0.78%;总磷水平分别为0.35%、0.67%和1.05%;NPP水平分别为0.07%、0.39%和0.77%(实测值)。

1.3 测定指标

1.3.1 肠道指数

试验第14天,每个重复选取1只体重相近的试验鹅进行屠宰。屠宰后,将肠道取出并分离,分别测量十二指肠、空肠和回肠长度。去除肠道表面脂肪以及肠道内的食糜,称量各肠段重量。

肠道相对长度(cm/g)=肠道绝对长度(cm)/体重(g);

肠道相对重量(g/g)=肠道绝对重量(g)/体重(g)。

1.3.2 肠道组织结构

试验第14天,每个重复选取1只体重相近的试验鹅进行屠宰解剖。将肠道表面脂肪清理干净,分别取十二指肠近端5 cm处、空肠和回肠中段约1 cm的肠段,用生理盐水冲洗肠道内容物后将各肠段放入4%甲醛固定液中保存,具体操作过程参考刘慧军等[14]。切片制作完成后观察并测量肠道绒毛长度、隐窝深度和肌层厚度。

1.3.3 食糜酶活性

试验第14天,每个重复选取1只体重相近的试验鹅进行屠宰解剖。分别取14日龄仔鹅的十二指肠、空肠黏膜作为试验样本,测定其碱性磷酸酶和Na+-K+ ATP酶的活性。测定所采用的试剂盒均购自南京建成生物工程研究所,测定步骤参照相应试剂盒说明书。

1.3.4 16S rRNA基因的高通量测序与分析

由于磷主要是在空肠中进行吸收转运,与空肠中的微生物有最直接的接触,故而本研究选择对空肠内容物进行16S rRNA基因的高通量测序。去除空肠表面的脂肪,取2 cm左右空肠内容物作为试验样本。将试验样本放入EP管,-80 ℃保存。用于分析空肠内容物菌群组成及结构。样本送至上海派森诺生物科技股份有限公司进行高通量测序分析。测序区域名称:16SV3V(a),目标片段长度:480 bp。分析流程:首先对高通量测序的原始下机数据根据序列质量进行初步筛查;对于问题样本重测、补测。通过质量初筛的原始序列按照index和Barcode信息,进行文库和样本划分,并去除barcode序列。按照QIIME2 dada2分析流程进行序列去噪。对不同组的样本在不同物种分类学水平的具体组成进行展示。

1.4 数据处理

采用SPSS 18.0软件对数据进行单因素方差分析,当方差分析结果显著时,采用Duncan氏法进行多重比较。数据结果用平均值和均值标准误(SEM)表示,P<0.05为差异显著。

2 结果与分析

2.1 饲粮NPP水平对仔鹅肠道形态的影响

2.1.1 对仔鹅肠道指数的影响

表1所示,LP组十二指肠、空肠和回肠的绝对长度显著低于CP组和HP组 (P<0.05);LP组肠道相对长度均显著高于CP组和HP组(P<0.05);LP组肠道的绝对重量显著低于CP组和HP组(P<0.05),CP组回肠绝对重量显著高于其他组(P<0.05);HP组空肠和回肠的相对重量显著低于LP组和CP组(P<0.05)。
表1 饲粮NPP水平对14日龄江南白鹅肠道指数的影响

Table 1 Effects of dietary NPP levels on intestinal indexes of Jiangnan white geese at 14 days of age

项目
Items
肠道
Intestine
低磷组
LP group
对照组
CP group
高磷组
HP group
SEM P
P-value


绝对长度
Absolute length/cm
十二指肠 Duodenum 23.77b 28.72a 28.25a 0.74 <0.01
空肠 Jejunum 51.02b 65.00a 61.72a 1.83 <0.01
回肠 Ileum 49.32b 62.15a 56.67a 1.81 <0.01
十二指肠 Duodenum 5.56a 3.91b 3.07c 0.26 <0.01

相对长度
Relative length/(cm/g)
空肠 Jejunum 11.98a 8.85b 6.71c 0.58 <0.01
回肠 Ileum 11.57a 8.46b 6.16c 0.58 <0.01
十二指肠 Duodenum 3.82b 6.16a 6.26a 0.41 0.01

绝对重量
Absolute weight/g
空肠 Jejunum 9.09b 15.90a 13.87a 0.80 <0.01
回肠 Ileum 9.41c 16.09a 13.11b 0.83 <0.01
十二指肠 Duodenum 0.89 0.84 0.68 0.05 0.22
相对重量
Relative weight/(g/g)
空肠 Jejunum 2.13a 2.17a 1.51b 0.10 <0.01
回肠 Ileum 2.20a 2.19a 1.43b 0.13 <0.01

同行数据肩标不同字母表示差异显著(P<0.05)。下表同。

In the same row, values with different letter superscripts mean significant difference (P<0.05). The same as bellow.

2.1.2 对仔鹅肠道组织结构的影响

表2所示,饲粮中添加NPP对14日龄江南白鹅的肠道组织结构并无显著影响(P>0.05),各肠段之间肠道的绒毛长度、隐窝深度、肌层厚度和绒隐比并无显著差异(P>0.05)。
表2 饲粮NPP水平对14日龄江南白鹅肠道组织结构的影响

Table 2 Effects of dietary NPP levels on intestinal morphology of Jiangnan white geese at 14 days of age

肠道
Intestine
项目
Items
低磷组
LP group
对照组
CP group
高磷组
HP group
SEM P
P-value


十二指肠
Duodenum
绒毛长度 Villus length/μm 784.22 910.23 865.45 29.00 0.21
隐窝深度 Crypt depth/μm 250.90 252.19 221.87 11.80 0.54
绒隐比 Villus length/crypt depth 3.56 3.49 3.51 0.23 0.99
肌层厚度 Muscle layer thickness/μm 243.26 271.93 276.00 10.17 0.41
绒毛长度 Villus length/μm 866.85 948.09 950.84 47.35 0.75


空肠
Jejunum
隐窝深度 Crypt depth/μm 237.17 245.92 238.47 7.73 0.90
绒隐比 Villus length/crypt depth 3.66 3.90 4.04 0.22 0.81
肌层厚度 Muscle layer thickness/μm 223.94 247.12 249.92 8.89 0.47
绒毛长度 Villus length/μm 551.19 703.55 705.65 37.56 0.15


回肠
Ileum
隐窝深度 Crypt depth/μm 255.46 233.59 239.81 6.20 0.38
绒隐比 Villus length/crypt depth 2.18 2.81 2.96 0.16 0.09
肌层厚度 Muscle layer thickness/μm 219.91 266.65 280.86 6.20 0.46

2.2 饲粮NPP水平对仔鹅肠道碱性磷酸酶和Na+-K+ ATP酶活性的影响

表3所示,LP组十二指肠碱性磷酸酶活性显著低于HP组(P<0.05)。LP组回肠Na+-K+ ATP酶的活性显著低于CP组和HP组(P<0.05)。
表3 饲粮NPP水平对14日龄江南白鹅肠道碱性磷酸酶和Na+-K+ ATP酶活性的影响

Table 3 Effects of dietary NPP levels on intestinal alkaline phosphatase and Na+-K+-ATPase activities of Jiangnan white geese at 14 days of age

项目
Items
肠道
Intestine
低磷组
LP group
对照组
CP group
高磷组
HP group
SEM P
P-value

碱性磷酸酶
Alkaline phosphatase/(U/g prot)
十二指肠 Duodenum 534.76b 615.8ab 691.68a 26.31 0.04
空肠 Jejunum 634.64 627.78 616.46 24.29 0.96

Na+-K+ ATP酶
Na+-K+-ATPase/(U/mg prot)
十二指肠 Duodenum 3.28 4.36 4.38 0.23 0.08
空肠 Jejunum 5.17b 6.05a 6.91a 0.24 <0.01

2.3 饲粮NPP水平对仔鹅空肠微生物多样性的影响

2.3.1 序列数及操作分类单元(OTU)数量统计
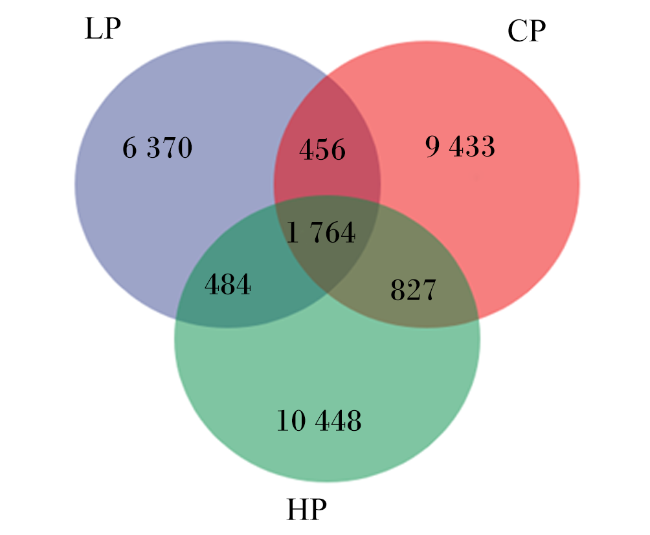
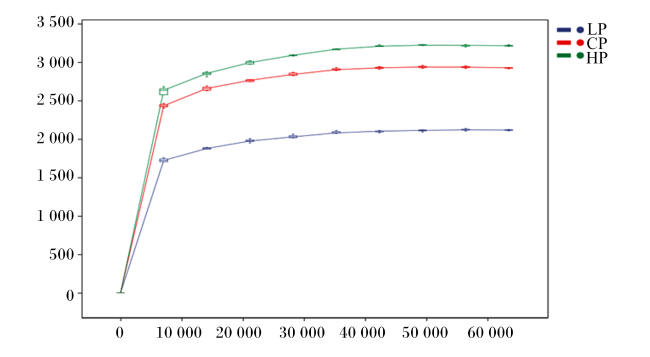
本试验对所有样本的有效序列,以97%的一致性进行OTU聚类,然后对OTU的序列进行物种注释。如图1所示,样品共检测出20 511个OTU,其中重复的OTU有3 531个,LP组有6 370个特有OTU,CP组有9 433个特有OTU,HP组有10 448个特有OTU。如图2所示,随着OTU数目的增大,所有组的曲线都趋于平缓,说明测序深度的增加不再影响菌种的鉴定,测序量合理。
图1 不同组特有和重复OTU数量花瓣图

LP、CP、HP分别表示低磷组、对照组、高磷组。下图同。

Fig.1 Petal diagram of unique and repetitive OTU numbers in different groups

LP, CP, HP indicated low phosphorus group, control group and high phosphorus group, respectively. The same as bellow.

图2 稀疏曲线

横坐标为序列数量,纵坐标为观察到的物种数量。

Fig.2 Sparse curve

The horizontal axis represents the number of sequences, and the vertical axis represents the number of observed species.

2.3.2 Alpha多样性分析

表4所示,LP组Chao1指数、Observed species指数、Shannon指数和Simpson指数显著低于CP组和HP组(P<0.05)。由此说明,LP组改变了空肠菌群的组成,其表征群落内物种分布的多样性和均匀度较低。
表4 饲粮NPP水平对14日龄江南白鹅空肠微生物Alpha多样性指数的影响

Table 4 Effects of dietary NPP levels on jejunal microbial Alpha diversity indexes of Jiangnan white geese at 14 days of age

项目
Items
低磷组
LP group
对照组
CP group
高磷组
HP group
SEM P
P-value
Chao1指数 Chao1 index 2 117b 2 923a 3 215a 178.98 0.02
Observed species指数Observed species index 2 019b 2 842a 3 089a 174.72 0.02
Shannon指数 Shannon index 9.12b 9.92a 9.93a 0.13 <0.01
Simpson指数 Simpson index 0.98b 1.00a 0.99a 0.001 <0.01

2.3.3 Beta多样性分析

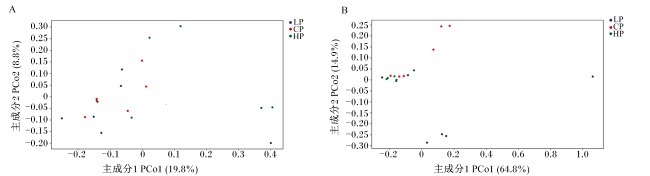
为了充分说明添加不同水平的NPP对14日龄江南白鹅空肠菌群的差异,本试验进行了Beta多样性分析,分析物种的系统发育关系和相对丰度。如图3所示,在加权Unifrac距离和非加权Unifrac距离的基础上进行主坐标分析(PCoA)。在非加权Unifrac主坐标分析中,第1个主成分(PCo1)解释了样本间19.8%的变化,第2个主成分(PCo2)解释了样本间8.8%的变化。而在加权Unifrac主坐标分子中,PCo1解释了样本间64.8%的变化,PCo2解释了样本间14.9%的变化。加权Unifrac距离不仅考虑了微生物菌群成员之间的系统发育,同时还考虑了微生物在各自的菌群中相对丰度的高低。从加权Unifrac中可以看出,LP组与其他2组相比物种变异较为明显。根据非加权Unifrac可知,CP组和HP组的物种比LP组更为丰富。
图3 基于饲粮中NPP水平的Beta多样性分析图

A:非加权Unifrac PCoA unweighted Unifrac PCoA;B:加权Unifrac PCoA weighted Unifrac PCoA。

Fig.3 Beta diversity analysis plot based on NPP levels in diets

2.3.4 属水平下的物种聚类分析

本试验在属水平下对微生物进行了物种聚类分析,如表5所示,LP组的代尔夫特菌属(Delftia)、苍白杆菌属(Ochrobactrum)、不动杆菌属(Acinetobacter)和黄杆菌属(Flavobacterium)相对丰度显著高于CP组和HP组(P<0.05)。同时,LP组中KD1-23、硝化螺旋菌属(Nitrospira)、囊裸藻属(Trachelomonas)和红育菌属(Rhodoferax)的相对丰度显著低于CP组和HP组(P<0.05)。
表5 饲粮NPP水平对14日龄江南白鹅空肠微生物属水平下前10菌群分布的影响

Table 5 Effects of dietary NPP levels on jejunal microbial distribution of top 10 flora at genus level of Jiangnan white geese at 14 days of age

项目
Items
低磷组
LP group
对照组
CP group
高磷组
HP group
SEM P
P-value
代尔夫特菌属 Delftia 0.060a 0.010b 0.010b 0.009 0 0.04
苍白杆菌属Ochrobactrum 0.050a 0.020b 0.010b 0.006 0 0.01
KD1-23 0.007b 0.012a 0.014a 0.000 9 <0.01
红细菌属Rhodobacter 0.008 0.010 0.010 0.000 6 0.08
硝化螺旋菌属Nitrospira 0.006b 0.008a 0.010a 0.000 6 <0.01
囊裸藻属Trachelomonas 0.006b 0.008a 0.009a 0.000 5 0.03
红育菌属 Rhodoferax 0.005b 0.008a 0.008a 0.000 6 0.03
动胶菌属 Zoogloea 0.006 0.007 0.008 0.000 4 0.07
不动杆菌属 Acinetobacter 0.010a 0.004b 0.003b 0.002 0 0.04
黄杆菌属Flavobacterium 0.010a 0.004b 0.005b 0.001 0 <0.01

2.3.5 门水平下的物种聚类分析

本试验在门水平下对微生物进行了物种聚类分析,如表6所示,变形菌门(Proteobacteria)、拟杆菌门(Bacteroidetes)和TM7为优势菌群。LP组的拟杆菌门、绿菌门(Chlorobi)和硝化螺旋菌门(Nitrospirae)的相对丰度显著低于CP组和HP组(P<0.05)。同时,LP组中TM7、厚壁菌门(Firmicutes)的相对丰度显著高于CP组和HP组(P<0.05)。这说明饲粮NPP水平会改变仔鹅空肠的菌群结构。
表6 饲粮NPP水平对14日龄江南白鹅空肠微生物门水平下前10菌群分布的影响

Table 6 Effects of dietary NPP levels on jejunal microbial distribution of top 10 flora at phylum level of Jiangnan white geese at 14 days of age

项目
Items
低磷组
LP group
对照组
CP group
高磷组
HP group
SEM P
P-value
变形菌门 Proteobacteria 0.490 0.510 0.520 0.007 3 0.35
拟杆菌门 Bacteroidetes 0.150b 0.170a 0.170a 0.004 9 0.04
TM7 0.130a 0.080b 0.080b 0.007 9 <0.01
放线菌门 Actinobacteria 0.050 0.060 0.060 0.001 3 0.22
绿弯菌门 Chloroflexi 0.030 0.040 0.040 0.001 0 0.29
厚壁菌门 Firmicutes 0.030a 0.020b 0.020b 0.002 0 0.03
绿菌门 Chlorobi 0.010b 0.020a 0.020a 0.001 0 0.03
硝化螺旋菌门 Nitrospirae 0.006b 0.008a 0.010a 0.000 6 <0.01
芽单胞菌门Gemmatimonadetes 0.005 0.005 0.006 0.000 4 0.81
螺旋体门 Spirochaetes 0.003 0.004 0.004 0.000 3 0.16

3 讨论

3.1 饲粮NPP水平对仔鹅肠道发育的影响

肠道是家禽消化、吸收营养物质的重要场所,因此,家禽肠道的健康发育对家禽机体健康和生产性能十分重要[15]。同样,温静[3]的研究结果表明,适宜的磷水平可以提高草鱼的肠道长度和肠道重量。本试验结果表明,随着饲粮NPP水平的升高,仔鹅的肠道绝对长度随之增加;仔鹅的十二指肠和空肠绝对重量也随着饲粮NPP水平的升高而增加。
肠道内的绒毛长度、隐窝深度和绒隐比是反映肠道吸收能力的重要指标[16]。Hou等[17]报道,肠绒毛长度和隐窝深度与肠道吸收能力密切相关。因此,隐窝深度越浅、绒毛长度越长,肠道吸收能力越好。绒毛长度缩短、营养吸收面积减少,会影响动物对营养物质的吸收能力;隐窝深度加深则表示组织细胞更新速度较快,促进绒毛发育[18]。Xu等[19]的研究表明,饲粮中NPP水平对14日龄肉鸭十二指肠肌层厚度呈线性影响。本试验结果显示,饲粮NPP水平对14日龄仔鹅肠道的绒毛长度、隐窝深度和肠层厚度没有显著影响。

3.2 饲粮NPP水平对仔鹅肠道碱性磷酸酶和Na+-K+ ATP酶活性的影响

肠黏膜是动物机体抵御外界病原侵袭、维持肠道健康的重要屏障结构[20]。Goldberg等[21]认为,肠道碱性磷酸酶在维持肠黏膜完整和改善肠道功能上具有一定的作用。肠道碱性磷酸酶能够反映肠道发育情况以及小肠上皮细胞的吸收功能,能够减少肠道炎症的发生[22]。有研究发现,肠道碱性磷酸酶主要在十二指肠表达[23],在空肠和回肠的表达较低[24]。在本试验条件下,CP组和HP组十二指肠中碱性磷酸酶活性高于LP组。这说明饲粮中足量的NPP水平可促进肠道碱性磷酸酶的分泌,减少肠道炎症的发生,改善14日龄江南白鹅仔鹅的肠道功能。
Na+-K+ ATP酶又被称为钠钾泵,在维持细胞结构和细胞膜功能等方面有着十分重要的作用[25]。Na+-K+ ATP酶可以通过催化ATP水解供能,调节细胞渗透压,为营养物质的吸收提供动力。ATP是细胞内的一种高能磷酸化合物,含有2个高能磷酸键,因此磷是合成ATP的重要组成成分。Na+-K+ ATP酶活性的高低,可以反映出肠道对营养物质吸收能力的强弱[26]。在本试验中,随着饲粮NPP水平的增加,CP组和HP组空肠中Na+-K+ ATP酶的活性显著高于LP组,饲粮NPP水平对14日龄仔鹅十二指肠中Na+-K+ ATP酶的活性没有显著影响。
因此,饲粮中含有足量的NPP可能通过促进碱性磷酸酶和Na+-K+ ATP酶的活性,增加小肠营养物质吸收的能量供应和上皮细胞结构的完整度,可提高肠道对营养物质的吸收能力。

3.3 饲粮NPP水平对仔鹅空肠菌群结构的影响

肠道正常生理功能的维持,离不开肠道微生物。肠道微生物结构的改变,对肠道健康有正面影响也有负面影响[27]。有研究表明,磷对于细菌的生长和增殖十分重要,并参与细菌的代谢过程[28]。在本试验条件下,饲粮NPP水平对14日龄江南白鹅仔鹅空肠微生物的Alpha指数有显著影响。LP组的表征群落内物种分布的多样性和均匀度低于CP组和HP组。由此可以看出,低磷饲粮降低了Chao1指数、Observed species指数、Shannon指数和Simpson指数,影响肠道微生物物种的丰度以及多样性。
代尔夫特菌属、苍白杆菌属、不动杆菌属和黄杆菌属广泛分布于自然界,这些细菌都属于条件性致病菌[29-32]。有研究表明,代尔夫特菌属主要出现在免疫力低下、患有严重基础病的患者中[33]。苍白杆菌属拥有5个种,包括人苍白杆菌、中间苍白杆菌、假中间苍白杆菌、嗜血苍白杆菌和特瑞特西苍白杆菌[34]。人苍白杆菌可以引起苍白杆菌的感染,而人苍白杆菌具有致病性,不仅感染人类也可以感染动物[30]。Franci等[35]研究发现,由于手术的麻醉药被人苍白杆菌污染,从而导致健康犬在犬牙清垢手术后出现致命性休克。不动杆菌属易生长,可以大量繁殖,从而破坏动物机体内微生态平衡,导致免疫力下降[36]。黄杆菌属不仅存在于自然界中,还广泛存在于动物肠道或器官中[37-38]。在本试验中,LP组的致病菌代尔夫特菌属、苍白杆菌属、不动杆菌属和黄杆菌属相对丰度显著高于CP组和HP组。由此可以推测,低磷饲粮可能会降低仔鹅的免疫力、破坏微生态平衡,使仔鹅感染致病菌,从而导致仔鹅生产性能降低。KD1-23、硝化螺旋菌属、囊裸藻属和红育菌属多在水和土壤中分布。在本试验中,LP组的KD1-23、硝化螺旋菌属、囊裸藻属和红育菌属的相对丰度显著低于CP组和HP组。但这些细菌在仔鹅中的作用机制尚未明确,还需进一步的研究。
不同的微生物菌群组成对宿主体内平衡和正常代谢有重要影响[39]。变形菌门是细菌中最大的一个群体[40],也是肠道菌群中生态失调的标志物,Shin等[41]认为,变形菌门在肠道中大量出现可以反映出肠道微生物群落结构不稳定。在本试验中,变形菌门在各组中处于重要地位,而饲粮NPP水平并未影响变形菌门的相对丰度,较为稳定。多糖是拟杆菌门的主要能量来源,它们可利用多种膳食可溶性多糖,代谢产物主要是乙酸盐和丙酸盐[42],在微生物消化和营养吸收等方面有着十分重要的作用。贾慧君[43]在肉鸡上研究发现,饲粮中NPP水平在0.39%与0.45%组的拟杆菌丰度最大,且生产性能最佳。由此可以推测,拟杆菌门丰度升高可促进肉鸡的生长发育。糖杆菌门又被称为解糖微小寄生菌[44],是需要寄生在宿主细菌上生长的细菌[45],在土壤、海水、动物和人体的口腔、胃肠道等均有分布[46-49]。有研究表明,糖杆菌门对宿主细胞具有选择性,目前糖杆菌门的宿主细菌主要是放线菌属,一小部分为假丙酸杆菌属[50-51]。糖杆菌门对于宿主细菌的有利之处在于可以使宿主细菌更好的定植,增加定植部位的菌量[52];而其对宿主细菌的负面影响在于会导致宿主细胞生长和增殖过于缓慢,甚至死亡[45]。本试验中,LP组糖杆菌门相对丰度高于其他2组,而与之相关的宿主细菌放线菌门的相对丰度在各组之间并无显著差异。但LP组的放线菌门的相对丰度比其他2组低20%,因此推测,糖杆菌门对放线菌产生负面影响。厚壁菌门是肠道中最主要的菌群之一,也是最丰富的门之一[53]。厚壁菌门与拟杆菌门都是肠道内最主要的细菌,两者之间存在相互促进的共生关系,因此,2种细菌之间的比例也十分重要。本试验中,LP组的有害菌厚壁菌门相对丰度显著高于CP组和HP组。同时,LP组的厚壁菌门相对丰度升高,拟杆菌门相对丰度降低,可以看出饲粮NPP水平过低会增加有害菌比例,降低有益菌比例。这可能是导致仔鹅对生产性能降低的原因之一。

4 结论

仔鹅饲粮NPP水平过低可代偿性地增加肠道相对长度,但其造成的肠道功能性酶活性下降、空肠微生物菌群失衡可能是饲粮低磷水平导致仔鹅生长性能下降的重要原因。鹅可耐受高达0.80%的NPP且对仔鹅早期肠道发育、空肠微生物结构无不利影响。
[1]
HEYER C M E, WEISS E, SCHMUCKER S, et al. The impact of phosphorus on the immune system and the intestinal microbiota with special focus on the pig[J]. Nutrition Research Reviews, 2015, 28(1):67-82.

DOI PMID

[2]
谢南彬. 磷对幼建鲤生长性能、消化吸收功能、免疫功能和抗氧化能力的影响[D]. 硕士学位论文. 雅安: 四川农业大学, 2010.

XIE N B. Effects of dietary phosphorus on growth performance,functions of digestion,absorption,immune and antioxidative of juvenile Jian carp[D]. Master’s Thesis. Ya’an: Sichuan Agricultural University, 2010. (in Chinese)

[3]
温静. 磷对中期草鱼生长性能、肌肉品质、抗氧化能力和免疫功能的影响[D]. 硕士学位论文. 雅安: 四川农业大学, 2013.

WEN J. Effect of dietary phosphorus on growth performance,meat quality,antioxidative ability and immune function of young giass carp[D]. Master’s Thesis. Ya’an: Sichuan Agricultural University, 2013. (in Chinese)

[4]
黄学琴. 复合酶制剂对肉鸭生产性能、养分利用率及钙磷代谢的影响[D]. 硕士学位论文. 雅安: 四川农业大学, 2013.

HUANG X Q. Effects of enzyme complex on growth performance,nutrient utilization,calcium and phosphorus metabolism of ducks[D]. Master’s Thesis. Ya’an: Sichuan Agricultural University, 2013. (in Chinese)

[5]
JACELA J Y, DEROUCHEY J M, TOKACH M D, et al. Feed additives for swine:fact sheets-prebiotics and probiotics and phytogenics[J]. Journal of Swine Health and Production. 2010, 18:87-91.

[6]
ABBASI F, FAKHUR-UN-NISA T, LIU J, et al. Low digestibility of phytate phosphorus,their impacts on the environment, and phytase opportunity in the poultry industry[J]. Environmental Science and Pollution Research International. 2019, 26(10):9469-9479.

DOI

[7]
SHASTAK Y, RODEHUTSCORD M. Determination and estimation of phosphorus availability in growing poultry and their historical development[J]. World's Poultry Science Journal, 2013, 69(3):569-586.

DOI

[8]
ABDALLAH A, ZHANG P, ZHONG Q Z, et al. Application of traditional Chinese herbal medicine by-products as dietary feed supplements and antibiotic replacements in animal production[J]. Current Drug Metabolism, 2019, 20(1):54-64.

DOI PMID

[9]
WU X Z, WEN Z G, HUA J L. Effects of dietary inclusion of Lactobacillus and inulin on growth performance,gut microbiota,nutrient utilization,and immune parameters in broilers[J]. Poultry Science, 2019, 98(10):4656-4663.

DOI

[10]
MANN E, DZIECIOL M, METZLER-ZEBELI B U, et al. Microbiomes of unreactive and pathologically altered ileocecal lymph nodes of slaughter pigs[J]. Applied and Environmental Microbiology, 2014, 80(1):193-203.

DOI PMID

[11]
BORDA-MOLINA D, VITAL M, SOMMERFELD V, et al. Insights into broilers’gut microbiota fed with phosphorus,calcium,and phytase supplemented diets[J]. Frontiers in Microbiology, 2016, 7:2033.

[12]
PTAK A, BEDFORD M R, ŚWIATKIEWICZ S, et al. Phytase modulates ileal microbiota and enhances growth performance of the broiler chickens[J]. PLoS One, 2015, 10(3):e0119770.

DOI

[13]
LI N, HE J Y, CHEN H, et al. Effects of dietary phosphorus deficiency and high phosphorus content on the growth performance,serum variables,and tibia development in goslings[J]. Agriculture, 2022, 12(11):1908.

DOI

[14]
刘慧军, 杨海明, 胥蕾, 等. 畜禽肠道组织H.E.染色石蜡切片制作要点及关键技术[J]. 黑龙江畜牧兽医(上半月), 2018(8):206-210.

LIU H J, YANG H M, XU L, et al. Key points and techniques of H.E.staining and paraffin sectionin livestock and poultry intestines[J]. Heilongjiang Animal Science and Veterinary Medicine(First Half of the Month), 2018(8):206-210. (in Chinese)

[15]
UR RAHMAN S, KHAN S, CHAND N, et al. In vivo effects of Allium cepa L.on the selected gut microflora and intestinal histomorphology in broiler[J]. Acta Histochemica, 2017, 119(5):446-450.

DOI

[16]
王菊. 饲粮非植酸磷水平对肉鸭生产性能,消化功能和肠道屏障的影响[D]. 硕士学位论文. 雅安: 四川农业大学, 2019.

WANG J. Effects of dietary non-phytate phosphorus levels on performance,digestive function and intestinal barrier function in meat duck[D]. Master’s Thesis. Ya’an: Sichuan Agricultural University, 2019. (in Chinese)

[17]
HOU Y, WANG L, DING B, et al. Dietary alpha-ketoglutarate supplementation ameliorates intestinal injury in lipopolysaccharide-challenged piglets[J]. Amino Acids. 2010, 39(2):555-564.

DOI PMID

[18]
XU Z R, HU C H, XIA M S, et al. Effects of dietary fructooligosaccharide on digestive enzyme activities,intestinal microflora and morphology of male broilers[J]. Poultry Science, 2003, 82(6):1030-1036.

DOI

[19]
XU H M, DAI S J, ZHANG K Y, et al. Dietary phosphorus deficiency impaired growth,intestinal digestion and absorption function of meat ducks[J]. Asian-Australasian Journal of Animal Sciences, 2019, 32(12):1897-1906.

DOI

[20]
HURLEY B P, MCCORMICK B A. Intestinal epithelial defense systems protect against bacterial threats[J]. Current Gastroenterology Reports, 2004, 6(5):355-361.

PMID

[21]
GOLDBERG R F, AUSTEN W G J Jr, ZHANG X B, et al. Intestinal alkaline phosphatase is a gut mucosal defense factor maintained by enteral nutrition[J]. Proceedings of the National Academy of Sciences of the United States of America, 2008, 105(9):3551-3556.

DOI PMID

[22]
万军, 田忠, 姚柏宇, 等. 肠碱性磷酸酶在肠黏膜屏障中的作用[J]. 世界华人消化杂志, 2019, 27(23):1441-1445.

WAN J, TIAN Z, YAO B Y, et al. Role of intestinal alkaline phosphatase in intestinal mucosal barrier[J]. World Chinese Journal of Digestology, 2019, 27(23):1441-1445. (in Chinese)

DOI

[23]
NARISAWA S, HUANG L, IWASAKI A, et al. Accelerated fat absorption in intestinal alkaline phosphatase knockout mice[J]. Molecular and Cellular Biology, 2003, 23(21):7525-7530.

DOI PMID

[24]
MOLNÁR K, VANNAY A, SZEBENI B, et al. Intestinal alkaline phosphatase in the colonic mucosa of children with inflammatory bowel disease[J]. World Journal of Gastroenterology, 2012, 18(25):3254-3259.

DOI PMID

[25]
孙进一. 星形胶质细胞钠钾泵在局灶性皮质发育不良癫痫中的作用研究[D]. 硕士学位论文. 杭州: 浙江大学, 2023.

SUN J Y. The role of astrocyte Na+-K+-ATPase in the epilepsy model with focal cortical dysplasia[D]. Master’s Thesis. Hangzhou: Zhejiang University, 2023. (in Chinese)

[26]
RHODAS J M, CHEN W, CHU P, et al. L-glutamine and L-asparagine stimulate Na+-H+ exchange in porcine jejunal enterocytes[J]. The American Journal of Physiology, 1994, 266(5 Pt 1):G828-G838.

[27]
GABRIEL I, LESSIRE M, MALLETT S, et al. Microflora of the digestive tract:critical factors and consequences for poultry[J]. World’s Poultry Science Journal, 2006, 62(3):499-511.

[28]
DURAND M, KOMISARCZUK S. Influence of major minerals on rumen microbiota[J]. The Journal of Nutrition, 1988, 118(2):249-260.

DOI

[29]
KHAN S, SISTLA S, DHODAPKAR R, et al. Fatal delftia acidovorans infection in an immunocompetent patient with empyema[J]. Asian Pacific Journal of Tropical Biomedicine, 2012, 2(11):923-924.

DOI PMID

[30]
刘志国, 崔步云, 夏咸柱. 人苍白杆菌研究进展[J]. 微生物学报, 2015, 55(8):977-982.

LIU Z G, CUI B Y, XIA X Z. Research progress of Ochrobactrum anthropic-a review[J]. Acta Microbiologica Sinica, 2015, 55(8):977-982. (in Chinese)

[31]
缪应纯, 徐晓林, 缪应举, 等. 鲍曼不动杆菌研究进展[J]. 山东化工, 2017, 46(23):49-51.

MIAO Y C, XU X L, MIAO Y J, et al. The research progress in Acinetobacter baumannii[J]. Shandong Chemical Industry, 2017, 46(23):49-51. (in Chinese)

[32]
刘欢. 黄杆菌属等三株新种的分离和多相分类研究[D]. 硕士学位论文. 南京: 南京农业大学, 2008.

LIU H. Studies on isolation and polyphasic taxonomy of Flavobacterium and other three new species[D]. Master’s Thesis. Nanjing: Nanjing Agricultural University, 2008. (in Chinese)

[33]
何露露. 生物膜反应器和一株代尔夫特菌脱氮特性研究[D]. 硕士学位论文. 武汉: 华中农业大学, 2014.

HE L L. Nitrogen removal of biofilim reactor and a delftia strain[D]. Master’s Thesis. Wuhan: Huazhong Agricultural University, 2014. (in Chinese)

[34]
周庭银. 临床微生物学诊断与图解[M]. 3版. 上海: 上海科学技术出版社, 2012.

ZHOU T Y. Diagnosis and illustration of clinical microbiology[M]. 3rd ed. Shanghai: Shanghai Scientific and Technical Publishers, 2012. (in Chinese)

[35]
FRANCI P, DOTTO G, CATTAI A, et al. Lethal septic shock after dental scaling in a healthy dog due to Ochrobactrum anthropi-contaminated propofol[J]. The Journal of Small Animal Practice, 2015, 56(5):345-347.

DOI

[36]
马全萍, 张倩, 孙玉国, 等. 鲍曼不动杆菌的临床分布及耐药变化趋势[J]. 现代预防医学, 2015, 42(23):4412-4413,4416.

MA Q P, ZHANG Q, SUN Y G, et al. Clinical distribution and drug resistance trend of Acinetobacter baumannii[J]. Modern Preventive Medicine, 2015, 42(23):4412-4413,4416. (in Chinese)

[37]
DUMAN M, AY H, ALTUN S, et al. Flavobacterium muglaense sp.nov.isolated from internal organs of apparently healthy rainbow trout[J]. International Journal of Systematic and Evolutionary Microbiology, 2021, 71(7):004903.

[38]
KANG S, LEE J Y, HAN J E, et al. Description of Flavobacterium cyclinae sp.nov.and flavobacterium channae sp.nov.,isolated from the intestines of Cyclina sinensis (corb shell) and Channa argus (northern snakehead)[J]. Journal of Microbiology, 2022, 60(9):890-898.

DOI

[39]
HOLMES E, LI J V, MARCHESI J R, et al. Gut microbiota composition and activity in relation to host metabolic phenotype and disease risk[J]. Cell Metabolism. 2012, 16(5):559-564.

DOI PMID

[40]
EMERSON D, RENTZ J A, LILBURN T G, et al. A novel lineage of proteobacteria involved i-n formation of marine Fe-oxidizing microbial mat communities[J]. PLoS One, 2007, 2(7):e667.

DOI

[41]
SHIN N R, WHON T W, BAE J W. Proteobacteria:microbial signature of dysbiosis in gut microbiota[J]. Trends in Biotechnology, 2015, 33(9):496-503.

DOI

[42]
THOMAS F, HEHEMANN J H, REBUFFET E, et al. Environmental and gut Bacteroidetes:the food connection[J]. Frontiers in Microbiology, 2011, 2:93.

[43]
贾慧君. 饲粮非植酸磷水平对1-21 d肉鸡生产性能、免疫功能及盲肠微生物菌群的影响[D]. 硕士学位论文. 雅安: 四川农业大学, 2018.

JIA H J. Effect of dietary non-phytate phosphorus levels on growth performance,immune function,and caecum microflora in broilers from 1 to 21 days of age[D]. Master’s Thesis. Ya’an: Sichuan Agricultural University, 2018. (in Chinese)

[44]
RHEIMS H, SPRÖER C, RAINEY F A, et al. Molecular biological evidence for the occurrence of uncultured members of the actinomycete line of descent in different environments and geographical locations[J]. Microbiology, 1996, 142(Pt 10):2863-2870.

DOI

[45]
聂杰, 陈宇星, 姜淞, 等. 解糖微小寄生茵的研究进展[J]. 中国科学(生命科学), 2021, 51(11):1523-1531.

NIE J, CHEN Y X, JIANG S, et al. Research progress of Saccharibacteria:a review[J]. Science in China(Life Sciences), 2021, 51(11):1523-1531. (in Chinese)

[46]
BIK E M, LONG C D, ARMITAGE G C, et al. Bacterial diversity in the oral cavity of 10 healthy individuals[J]. The ISME Journal, 2010, 4(8):962-974.

DOI

[47]
FREDRICKS D N, FIEDLER T L, MARRAZZO J M. Molecular identification of bacteria associated with bacterial vaginosis[J]. The New England Journal of Medicine, 2005, 353(18):1899-1911.

DOI PMID

[48]
GRICE E A, SEGRE J A. The skin microbiome[J]. Nature Reviews.Microbiology, 2011, 9(4):244-253.

[49]
BOR B, COLLINS A J, MURUGKAR P P, et al. Insights obtained by culturing saccharibacteria with their bacterial hosts[J]. Journal of Dental Research, 2020, 99(6):685-694.

DOI PMID

[50]
COLLINS A J, MURUGKAR P P, DEWHIRST F E. Complete genome sequence of strain AC001,a novel cultured member of the human oral microbiome from the candidate phylum Saccharibacteria (TM7)[J]. Microbiology Resource Announcements, 2019, 8(42):e01158-19.

[51]
BEDREE J K, BOR B, CEN L, et al. Quorum sensing modulates the epibiotic-parasitic relationship between Actinomyces odontolyticus and its Saccharibacteria epibiont,a nanosynbacter lyticu strain,TM7x[J]. Frontiers in Microbiology, 2018, 9:2049.

DOI

[52]
刘苗苗, 毕冉冉, 孙玉敬. 果蔬与肠道菌群互作及其健康功效研究进展[J]. 中国食品学报, 2022, 22(4):387-407.

LIU M M, BI R R, SUN Y J. Recent advances on the interaction between fruits or vegetables and intestinal flora and its effect on health[J]. Journal of Chinese Institute of Food Science and Technology, 2022, 22(4):387-407. (in Chinese)

[53]
陈说, 张帆, 范艳飞, 等. 膳食胆酸对营养性肥胖大鼠肠道炎症的改善及对肠道菌群中拟杆菌门与厚壁菌门比例的影响[J]. 胃肠病学和肝病学杂志, 2022, 31(10):1126-1131.

CHEN S, ZHANG F, FAN Y F, et al. Dietary bile acid improves intestinal inflammation in nutritionally obese rats and its effect on the ratio of Bacteroides and Firmicutes in the intestinal flora[J]. Chinese Journal of Gastroenterology and Hepatology, 2022, 31(10):1126-1131. (in Chinese)

文章导航

/