综述

Kelech样环氧氯丙烷相关蛋白1-核因子E2相关因子2-抗氧化反应元件信号通路及其激活剂在畜禽生产中应用的研究进展

  • 张朝生 ,
  • 陈志敏 , * ,
  • 王少龙 ,
  • 刘国华
展开
  • 中国农业科学院饲料研究所,农业农村部生物饲料重点实验室,北京 100081
* 陈志敏,副研究员,硕士生导师,E-mail:

张朝生(1998—),女,河北邯郸人,硕士研究生,从事动物营养与饲料科学研究。E-mail:

Office editor: 菅景颖

收稿日期: 2023-11-27

  网络出版日期: 2024-05-15

基金资助

中国农业科学院创新工程(CAAS-ASTIP-2023-IFR-10)

Research Progress of Kelech-Like Epichlorohydrin-Associated Protein 1-Nuclear Factor E2-Related Factor 2-Antioxidant Response Element Signaling Pathway and Application of Its Activators in Livestock and Poultry Production

  • ZHANG Chaosheng ,
  • CHEN Zhimin , * ,
  • WANG Shaolong ,
  • LIU Guohua
Expand
  • Key Laboratory for Feed Biotechnology of the Ministry of Agriculture and Rural Affairs, Institute of Feed Research of Chinese Academy of Agriculture Sciences, Beijing 100081, China
* associate professor, E-mail:

Received date: 2023-11-27

  Online published: 2024-05-15

摘要

Kelech样环氧氯丙烷相关蛋白1-核因子E2相关因子2-抗氧化反应元件(Keap1-Nrf2-ARE)是调控动物体内多种抗氧化酶和Ⅱ相解毒酶表达的信号通路,在氧化应激反应中发挥着重要作用。研究发现,益生菌和植物提取物具有良好的抗氧化活性,作为激活剂能够激活动物体内Keap1-Nrf2-ARE信号通路,从而增强机体的抗氧化能力,缓解机体的氧化应激反应,并提高畜禽生长性能。本文首先阐述了Keap1-Nrf2-ARE信号通路各部分的基本结构和功能,然后分析了Keap1-Nrf2-ARE信号通路在机体氧化应激反应中的调控机制,最后对能够激活Keap1-Nrf2-ARE信号通路的激活剂进行了分类总结并概述了其在畜禽生产中应用的研究进展,旨在为畜牧领域新型饲料添加剂的研发以及缓解机体氧化应激的深入研究提供参考。

本文引用格式

张朝生 , 陈志敏 , 王少龙 , 刘国华 . Kelech样环氧氯丙烷相关蛋白1-核因子E2相关因子2-抗氧化反应元件信号通路及其激活剂在畜禽生产中应用的研究进展[J]. 动物营养学报, 2024 , 36(5) : 2813 -2829 . DOI: 10.12418/CJAN2024.243

Abstract

Kelech-like epichlorohydrin-associated protein 1-nuclear factor E2-related factor 2-antioxidant response element (Keap1-Nrf2-ARE) is a signaling pathway that regulates the expression of various antioxidant enzymes and Ⅱ phase detoxification enzymes in animals, and plays an important role in oxidative stress response. Studies have found that a variety of probiotics and plant extracts with outstanding antioxidant activity can be used to activate the Keap1-Nrf2-ARE signaling pathway in animals, consequently enhancing the antioxidant capacity of the body, alleviating the oxidative stress response of the body, and improving the growth performance of livestock and poultry. This review described the basic molecular structure of each part of Keap1-Nrf2-ARE signaling pathway, and the regulatory mechanism of Keap1-Nrf2-ARE signaling pathway in oxidative stress response, and also summarized the activators that can activate Keap1-Nrf2-ARE signaling pathway, and the research progress of Keap1-Nrf2-ARE activators applied in livestock and poultry production. Based on our collected findings, we aimed to provide a reference for the development of new feed additives in the field of animal husbandry and further study on alleviating oxidative stress in animals.

随着畜禽集约化养殖模式的深入发展,畜禽面临着高密度、致病菌增多、高温等多种应激源的侵扰。这些应激源会引起体内的活性氧(ROS)和自由基大量积累,破坏了自由基产生与清除的平衡,导致机体出现氧化应激状态[1-2],促使畜禽发生肠道损伤、免疫抑制、代谢性疾病等,严重影响畜禽的生长发育[3-5]。Kelech样环氧氯丙烷相关蛋白1-核因子E2相关因子2-抗氧化反应元件(Keap1-Nrf2-ARE)信号通路调控一系列解毒和抗氧化酶基因的表达,在维持ROS产生和消除之间的平衡起着重要作用。益生菌和植物中存在的一些活性物质能够调节Nrf2介导的Ⅱ相解毒酶,进而缓解氧化应激,提高畜禽生长性能和改善肉品质[6-10]

1 Keap1-Nrf2-ARE信号通路的结构和功能

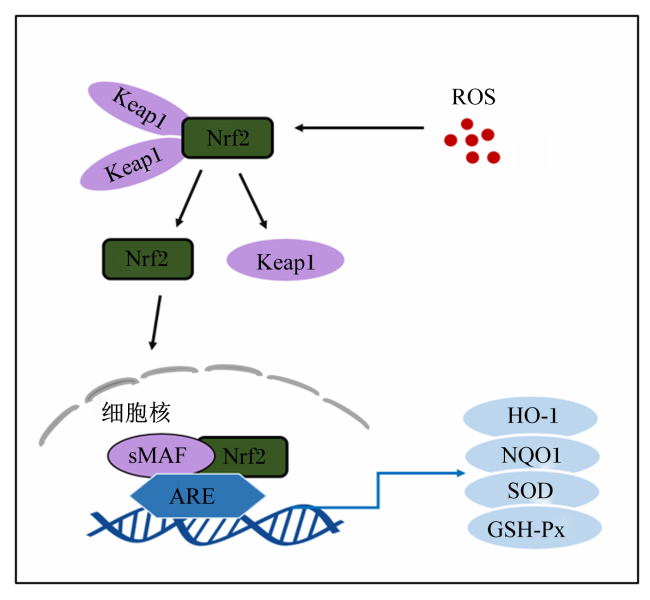
Keap1-Nrf2系统是一种进化上保守的防御系统,是细胞对环境胁迫反应的主要调节因子,其调控机制包括应激感知、基于蛋白酶体的Nrf2活性调控和靶基因的选择[11]。Nrf2与ARE相结合调节抗氧化相关酶的表达,是机体氧化应激防御系统的重要调节因子[12]。在正常生理状态下,Nrf2存在于细胞质中,但当细胞处于氧化应激状态时,Nrf2转移到细胞核内与ARE结合,启动下游血红素氧化酶-1(hemeoxygenase-1,HO-1)、NAD(P)H-醌氧化还原酶1[NAD(P)H:quinone oxidoreductase 1,NQO1]、谷胱甘肽过氧化物酶(glutathione peroxidase,GSH-Px)、超氧化物歧化酶(superoxide dismutase,SOD)等抗氧化酶基因的转录,从而提高细胞的抗氧化能力(图1)[13-14]
图1 Keap1-Nrf2-ARE信号通路整体路线机制图

ROS:活性氧 reactive oxygen species;Keap1:Kelech样环氧氯丙烷相关蛋白1 Kelch-like ECH-associated protein 1;Nrf2:核因子E2相关因子2 nuclear factor erythroid 2-related factor 2;sMAF:小MAF small MAF;ARE:抗氧化反应元件 antioxidant response element;HO-1:血红素氧化酶-1 hemeoxygenase-1;NQO1:NAD(P)H-醌氧化还原酶1 NAD(P)H:quinone oxidoreductase 1;SOD:超氧化物歧化酶 superoxide dismutase;GSH-Px:谷胱甘肽过氧化物酶 glutathione peroxidase。下图同 the same as below。

Fig.1 Overall routing mechanism diagram of Keap1-Nrf2-ARE signaling pathway[13-14]

1.1 Keap1的基本结构和功能

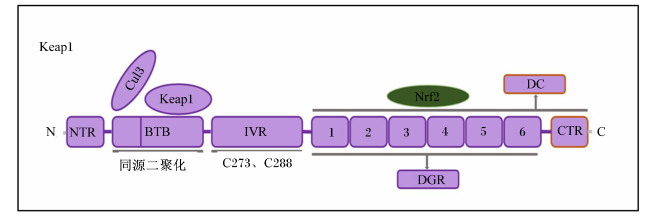
Keap1由624个氨基酸组成,分子质量为69 kD,是一种应激传感器蛋白,有助于Nrf2的快速降解,且直接与泛素连接酶Cullin3(Cul3)结合,形成泛素-蛋白连接酶(ubiquitin-protein ligating enzyme,E3)[15]。Keap1的三级结构完整才能介导Nrf2的泛素化,Keap1由5个主要结构域组成(图2),从N端到C端依次是N端序列结构域(N-terminal region,NTR)、BTB(broad-complex, tramtrack, and bric-a-brac)结构域、干预结构域(intervening region,IVR)、双甘氨酸重复区(double glycine repeat,DGR)或Kelch结构域和C端序列结构域(C-terminal region,CTR)[16-17]。每一个区域都有固定的功能,并在Keap1活动中起着不可或缺的作用。BTB结构域有关于Keap1的同源二聚化,包含半胱氨酸残基,促使Keap1-Nrf2解离和阻止Ⅱ相抗氧化酶转录[18]。IVR在与Cul3结合和支持Nrf2泛素化所需的连接酶复合物E3方面具有重要作用,含有关键的亲电反应部位半胱氨酸C273和C288,半胱氨酸的共价修饰引起Keap1的变化,干扰Nrf2泛素化和降解,增加了Nrf2水平和使细胞起保护反应,并且突变在体内引起组成型Nrf2活化[19-20]。DC(D-甘氨酸重复序列或Kelch结构域加C端结构域)是由DGR的6个双链甘氨酸重复序列和CTR组合形成的含有多个特定蛋白质结合位点,与Nrf2的Neh2结构域中低亲和力的DLG基序和高亲和力的ETGE基序相互作用来激活通路[21-22]
图2 Keap1的结构

NTR:N端序列结构域 N-terminal region;Cul3:Cullin3;BTB:broad-complex, tramtrack, and bric-a-brac;IVR:干预结构域 intervening region;DGR:双甘氨酸重复区 double glycine repeat;CTR:C端序列结构域 C-terminal region。

Fig.2 Structure of Keap1[23]

1.2 Nrf2的基本结构和功能

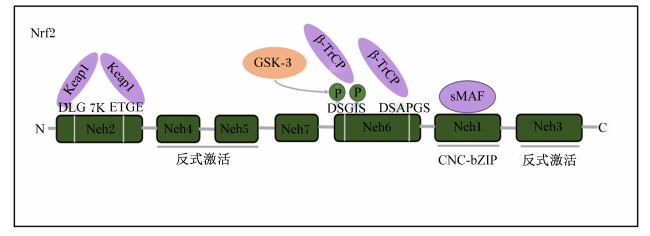
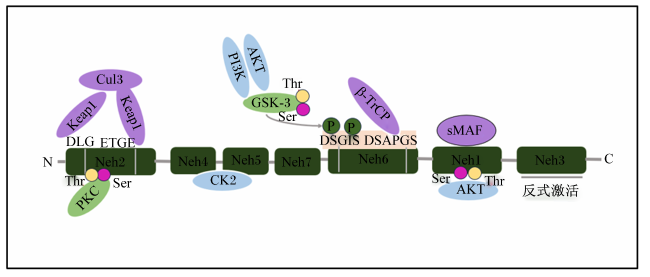
Nrf2由605个氨基酸构成的7个高度保守的同源结构域Neh组成(图3)[23-25],其分子质量为67.8 kD,是活力最强的帽和领(cap‘n’collar,CNC)氧化还原敏感性转录因子蛋白。Nrf2具有调节线粒体生物能量[26]、蛋白酶体活性和氧化应激[24]的生物学功能,在氧化应激期间主导ARE驱动的Ⅱ期基因的调节[27-28],所以称为应激反应的主要调节因子[29]。组成Nrf2的结构域从N端到C端是依次Neh2、Neh4、Neh5、Neh7、Neh6、Neh1和Neh3结构域,每个结构域具有不同的功能。Neh2结构域通过低亲和力DLG基序和高亲和力ETGE基序这2个高度保守的氨基酸片段介导与Keap1的相互作用,其中DLG基序具有三螺旋结构,与Keap1-DC结构域弱结合,而ETGE基序是单个β发夹结构,以钥匙和锁定方式与Keap1-DC结构域紧密结合;DLG基序和ETGE基序中间存在赖氨酸残基(7K)的亲水区,其调节Keap1依赖性泛素化和Nrf2降解,是氧化还原敏感的降解决定子,和维持Nrf2的表达量,使其稳定存在于细胞质中[30-31];Neh4和Neh5是Nrf2中2个独立的反式激活结构域,以氧化应激非依赖性方式协同结合激活剂环腺苷酸反应元件结合蛋白(cAMP response element binding protein,CREB)的结合蛋白(CBP)以激活Nrf2启动转录功能[32];Neh5与染色质重塑复合物的催化亚基BRG1(brahma-related gene 1)结合促进Z-DNA形成和聚集RNA聚合酶Ⅱ,在Nrf2介导的HO-1诱导表达中至关重要[33];Neh7结构域与视黄醇类X受体α(retinoid X receptor alpha,RXRα)相互作用的区域,二者结合后可抑制Nrf2的活性[34];Neh6结构域是一个富含丝氨酸的区域,包含2个保守的肽基序被β转导的重复蛋白(β-transducing repeat-containing protein,β-TrCP)识别控制,通过操控糖原合酶激酶-3(glycogen synthase kinase-3,GSK-3)活性来增加和减少[35],是细胞核中另一个降解决定子,调节Nrf2的稳定性的负调控[36]。Neh1包含异二聚化的CNC-碱性亮氨酸拉链(basic leucine zipper,bZIP)域,具有DNA结合域,可以与小Maf(small Maf,sMAF)蛋白结合形成二聚体[37]。sMAF蛋白具有亮氨酸拉链(ZIP)结构域,是与bZIP转录因子形成同源二聚体或异二聚体的复合物。Neh3是Nrf2的C端结构域,具有反式激活活性,与Neh4和Neh5结构域协同激活Nrf2靶基因,同时与染色体结构域解旋酶DNA结合蛋白6(CHD6)相互作用,使Nrf2具有活性[38]。缺失和突变的不完整Neh2结构域使Nrf2蛋白不能激活ARE依赖性基因表达,Nrf2对于完整的Ⅱ期代谢是必不可少的[39-41]
图3 Nrf2的结构

GSK-3:糖原合酶激酶-3 glycogen synthase kinase 3;β-TrCP:β转导的重复蛋白 β-transducing repeat-containing protein; CNC-bZIP:CNC-碱性亮氨酸拉链 CNC-basic leucine zipper。下图同 the same as below。

Fig.3 Structure of Nrf2[23]

Nrf2调控序列位于编码Ⅱ期解毒酶的基因上游,调控其基因的解毒功能[42-43],可以消除Ⅰ期反应产生的中间代谢物,加速有毒异生素的排泄[44]。因在抗氧化基因的上游存在ARE序列,所以Nrf2是氧化应激反应的主要调节因子[45]。Nrf2的靶基因调控谷胱甘肽、抗氧化蛋白酶、药物代谢酶和转运蛋白的基因表达,激活广泛的细胞防御过程,从而增强细胞解毒和将有害物质排除体外的能力。

1.3 ARE的基本结构和功能

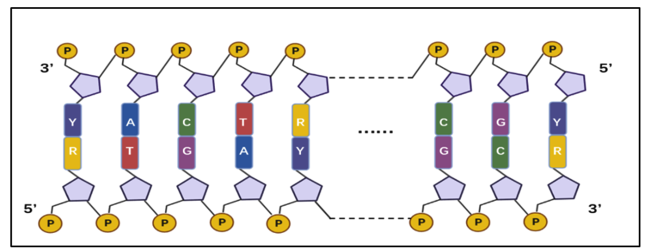
ARE是Telakowski-Hopkins等[46]在对大鼠体内谷胱甘肽S-转移酶(glutathione S-transferase,GST)Ya亚基结构基因的启动区进行功能分析时发现的。ARE是机体内重要的保护性顺式应答元件,是抗氧化蛋白和许多Ⅱ相解毒酶基因上游核心保护序列的转录调控因子,存在于大部分细胞保护基因的上游启动子区域的5’端,其核心序列(图4)为5’-(G/A)TGA(C/T)nnnGC(G/A)-3’(n为任意核苷酸),可与Nrf2等转录因子结合,调节细胞内与氧化还原平衡、Ⅱ相解毒酶、转运蛋白等相关基因,诱导HO-1等抗氧化酶基因的表达,缓解细胞或组织受到的各类损伤,维持机体内稳态的平衡[47]
图4 ARE的结构图

R=A或G;Y=C或T。R=A or G;Y=C or T.

Fig.4 Structure of ARE

2 Keap1-Nrf2-ARE信号通路的调节机制

Nrf2与ARE相结合可调节抗氧化相关酶的基因转录,是机体氧化应激防御系统的重要调节因子。Keap1-Nrf2-ARE可以分为两部分,一部分在细胞质,一部分在细胞核。

2.1 Nrf2泛素化
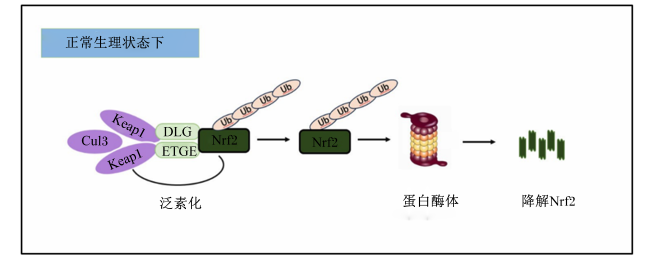
在正常生理状态下,Nrf2存在于细胞质中(图5),Keap1的IVR与Cul3(泛素连接酶)的N端区域特异性相互作用形成的E3[48-49]与Nrf2的Neh2结构域中低亲和力的DLG基序和高亲和力的ETGE基序介导相互作用,其中DLG基序具有三螺旋结构,与Keap1-DC结构域弱结合,而ETGE基序是单个β发夹结构,以钥匙和锁定方式与Keap1-DC结构域紧密结合,使Nrf2泛素化[30],进而通过蛋白酶体系快速降解,其中Keap1的BTB结构域和IVR是降解Nrf2的诱导泛素蛋白酶体因子[50]。因此,在非应激条件下Nrf2被不断合成,但又被快速降解而无活性。
图5 Nrf2泛素化的机制图

Fig.5 Schematic diagram of Nrf2 ubiquitination[48-49]

2.2 Nrf2与Keap1解偶联

在ROS应激条件下,Keap1的活性半胱氨酸残基被直接修饰[51],使其构象发生改变,这降低了Keap1-Cul3复合体E3的活性,从而抑制Nrf2的泛素化[52];Keap1-Nrf2二聚体解偶联后促使Nrf2易位进入细胞核,使Nrf2稳定增加与sMAF蛋白形成异二聚体,与抗氧化基因启动子中的ARE结合,刺激ARE的活化,启动下游HO-1、NQO1、GST、γ-谷氨酰半胱氨酸连接酶(γ-glutamate cysteine ligase,GCL)、GSH-Px、硫氧还蛋白还原酶(thioredoxin reductase,TrxR)、过氧化氢酶(catalase,CAT)、SOD等抗氧化应激活性物质基因的转录[53],提高抗氧化酶的表达量来清除自由基和过氧化产物,使氧化与抗氧化系统恢复平衡,减轻氧化损伤的程度[13,54](图6)。
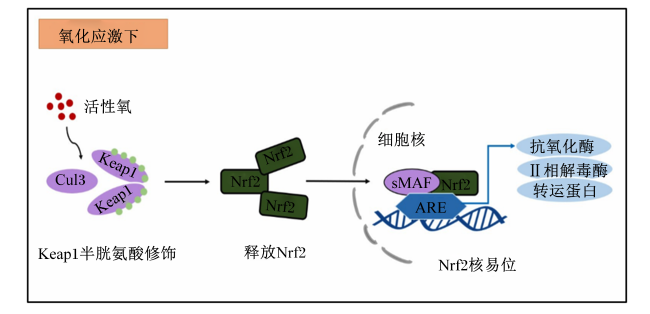
图6 Nrf2与Keap1解偶联的机制图

Fig.6 Schematic diagram of uncoupling Nrf2 and Keap1[52]

2.3 Nrf2直接磷酸化

从Nrf2的结构上看,含有很多氨基酸残基,存在大量的磷酸化位点(图7)。当一些氨基酸被磷酸化后可以影响Nrf2蛋白酶的活性、易位和与ARE的结合,从而调控氧化应激。蛋白激酶C(protein kinase C,PKC)具有多种亚型丝氨酸和苏氨酸激酶,可在Neh2结构域磷酸化Nrf2,导致Nrf2与Keap1解离,从而促进Nrf2的转录活性[55]。GSK-3是一种广泛表达的丝氨酸和苏氨酸激酶,可以对Neh6的DSGIS区域磷酸化,进而被β-TrCP识别诱导形成完整的E3,导致Neh6泛素化[56]。GSK-3抑制剂在一定条件下被用作Nrf2激活剂,磷脂酰肌醇-3-激酶(phosphoinositide-3-kinase,PI3K)/蛋白激酶B(protein kinase B,PKB或AKT)可以磷酸化GSK-3β阻断GSK-3的活性来促进Nrf2活性[57]。AMP活化蛋白激酶(AMP activated protein kinase,AMPK)是一种异源三聚体丝氨酸和苏氨酸激酶,直接磷酸化位点存在Neh1结构域内,促进了细胞中的Nrf2核积累[58]。酪蛋白激酶2(casein kinase 2,CK2)可磷酸化Nrf2的Neh4和Neh5结构域,诱导E3的活性,从而抑制Nrf2的泛素化,稳定了Nrf2的存在[59]
图7 Nrf2磷酸化

PKC:蛋白激酶C protein kinase C;CK2:酪蛋白激酶2 casein kinase 2;PI3K:磷脂酰肌醇-3-激酶 phosphoinositide-3-kinase;AKT:蛋白激酶B protein kinase B;Thr:苏氨酸 threonine;Ser:丝氨酸 serine。

Fig.7 Phosphorylation of Nrf2[23]

3 Keap1-Nrf2-ARE信号通路的功能

3.1 调节氧化应激

当氧化应激发生时,Keap1的活性半胱氨酸残基被直接修饰,降低了Keap1-Cul3复合体E3的活性,从而抑制Nrf2的泛素化,Nrf2转移到细胞核内与ARE结合,ARE被激活,调节下游抗氧化蛋白的产生[53],通过提高抗氧化酶的表达量来清除自由基和过氧化产物,使氧化与抗氧化系统恢复平衡,减轻氧化损伤的程度[54]。Wen等[60]研究表明,枯草芽孢杆菌通过上调仔猪回肠中Nrf2的蛋白表达,下调Keapl的蛋白表达,提高了肠道黏膜中抗氧化酶CAT、SOD和GSH-Px的活性,降低丙二醛(malondialdehyde,MDA)的含量,显著改变了肠道菌群的丰富度,进而减轻断奶仔猪肠道紊乱。王琳燚等[61]研究表明,肉鸡饲粮中添加金银花提取物通过调控胸肌中Nrf2基因表达,提高胸肌中SODGSH-Px基因的表达和降低MDA含量,进而提高胸肌的抗氧化性能,改善肉鸡胸肌肉品质。

3.2 抗炎

Nrf2在调节先天免疫应答、减少促炎基因表达和增强抗炎信号传导方面至关重要。血红素可被ARE表达的HO-1和环氧合酶-2(COX-2)催化降解为胆红素、一氧化碳(carbon monoxide,CO)和游离铁,其中CO作为核因子-κB(nuclear factor kappa-B,NF-κB)通路的抑制剂,导致促炎细胞因子的表达降低,而胆红素也起抗氧化作用[62]。同时,Nrf2的激活抑制巨噬细胞中促炎细胞因子[63]以及中性粒细胞中肿瘤坏死因子-α(tumor necrosis factor-α,TNF-α)、白细胞介素-6(interleukin-6,IL-6)和趋化因子CC型趋化因子配体2(CC chemokine ligand 2,CCL2)、CXC型趋化因子配体2(CXC chemokine ligand 2,CXCL2)的转录[64]。Wang等[65]研究表明,四黄止痢颗粒显著降低了促炎细胞因子TNF-α、白细胞介素-1β(interleukin-1β,IL-1β)和氧化应激标志物ROS、MDA含量,增加了体内抗炎细胞因子白细胞介素-4(interleukin-4,IL-4)、白细胞介素-10(interleukin-10,IL-10)含量和抗氧化酶GSH-Px、CAT活性,提高了鸡的免疫力。Ványolós等[66]研究表明,菌猴头菇提取物和甾体类化合物对COX-2具有显着的抑制特性,并且能够激活Nrf2途径达到抗炎效果。

3.3 治疗肝脏、肾脏损伤

Nrf2活化通过增加参与抗氧化防御的基因表达和减少参与脂肪生成的基因表达来防止酒精诱导的氧化应激和肝脏中游离脂肪酸的积累[67]。谭斅[68]研究表明,木犀草素显著提高了鹌鹑肝脏和肾脏中GSH含量、SOD活性以及Nrf2、HO-1和NQO1表达水平,进而缓解无机汞诱导的肝脏和肾脏损伤。陈诺等[69]研究表明,清肾颗粒(主要成分:生大黄、茵陈、黄连、白花蛇舌草、丹参、泽泻)激活大鼠肾脏组织中Nrf2,提高HO-1的表达量,减轻氧化应激反应,进而改善肾脏组织结构和功能。刘运华等[70]报道,糖肾宁(主要成分:熟地黄、山萸肉、怀山药、杜仲、炒白芍、淫羊藿、水蛭、酒大黄)通过调节大鼠体内HO-1的含量,促进体内抗氧化系统的激活,从而保护大鼠肾脏功能,降低血脂水平,减轻肾小管的氧化应激损伤。

3.4 维持血糖稳定

Nrf2可以调节脂质代谢相关基因表达,促进脂肪酸氧化和抑制脂肪生成,调控胰岛素分泌和胰岛素敏感组织中的葡萄糖利用,抑制糖异生,在维持葡萄糖代谢方面起重要作用[71]。Deng[72]研究发现,黄芪甲苷可激活患有糖尿病酮症酸中毒(DKA)的幼年小鼠的Nrf2通路,增强胰腺组织的抗氧化能力,缓解胰腺组织的损伤,提高胰岛素水平,缓解高血糖。孙梦雪等[73]研究指出,虫草发酵菌丝体通过增加大鼠肌肉、肝脏组织中Nrf2、HO-1和NQO1 mRNA的表达量,显著改善了大鼠空腹血糖、血脂和机体氧化应激水平。

4 Keap1-Nrf2-ARE信号通路激活剂的分类及其在畜禽生产中的应用

Keap1的功能主要由自身高活性硫醇基团发挥,这些基团能够通过氧化还原和烷基化被激活剂修饰[74]。Nrf2可被多种化合物激活,在氧化剂刺激下,ROS与Keap1的半胱氨酸残基结合导致构象变化,抑制Nrf2泛素化,促进Nrf2易位进入细胞核与ARE在抗氧化基因启动子中结合[75-76]。研究表明,在多种植物和益生菌中提取到的白藜芦醇、槲皮素、黄芩素、叶黄素、虾青素、番茄红素、表没食子儿茶素等活性物质都可以作为通路激活剂,激活Keap1-Nrf2-ARE信号通路[77-79]。研究还发现这些通路激活剂能够提高畜禽生长性能、改善肉品质和肠道微生物菌群[80-97](表1)。
表1 具有通路激活作用的活性物质在畜禽生产中的应用研究

Table 1 Application researches of active substances with pathway activation in livestock and poultry production

分类
Classifications
活性物质
Active
substances
研究对象
Objects of study
结果
Results
文献
References
多酚类
Polyphenols
白藜芦醇 仔猪 通过提高抗氧化酶活性、降低丙二醛
含量等来降低仔猪腹泻,提高其生长性能
[80]
通过激活核因子E2相关因子2(Nrf2)/血红素氧化酶-1(HO-1)
信号通路提高抗氧化能力和有效减轻肝炎和肝脏损伤,
最终显著提高鸭的平均日增重
[81]
儿茶素 肉鸡 通过增强抗氧化性能,减轻热应激引起的氧化
损伤,提高肉鸡的生长性能
[82]
肉鸡 通过提高肌肉抗氧化能力减少热应激对肝脏和空肠中
Nrf2表达的损害,进而改善肉鸡的肉质和肌肉氧化还原平衡
[83]
槲皮素 肉鸡 显著改善肠道菌群环境、提高抗氧化酶活性、增强
肠道形态和提高肉鸡的生长性能
[84]
断奶仔猪 调节机体代谢、促进有益菌增殖、改善
肠道健康,促进断奶仔猪的生长
[85]

黄芩素
减弱促炎细胞因子的水平和缓解
细胞凋亡,促进鸡的生长
[86]
蛋鸡 通过改善肠道微生物的组成来减轻肠道炎症和
屏障功能障碍,进而提高蛋鸡的生产性能
[87]
肉鸡 使肉鸡的体重和饲料转化率增加,
改善其生长性能和营养物质消化率
[88]
天然色素类
Natural
pigments

叶黄素
蛋鸡 增加产蛋率、生育力和孵化率,
提高蛋鸡的产蛋性能
[89]
肉鸡 显著提高皮肤颜色的黄色评分和胴体色素
沉着值,从而改善对肉鸡的肉色
[90]

虾青素
肉鸡 增强肉鸡在热应激期间的抗氧化防御系统,改善肉色和
质量,进而提高肉鸡的肉质、生长性能和免疫能力
[91]
肉鸡 显著提高肉鸡的平均体重、日增重、累计采食
量和饲料系数,并显著降低总死亡率
[92]
番茄红素 母猪 增加母猪的胎盘健康和乳成分,增加窝产仔数、
出生重和断奶窝重,提高母猪的繁殖性能
[93]
维生素及其
衍生物
Vitamins
and their
derivatives
α-硫辛酸 肉鸡 提高肉鸡平均日增重、终末体重、肠道绒毛高度
和绒毛高度与隐窝深度之比,同时改善盲肠中有益菌乳酸
杆菌的丰度,有效地减轻热应激对肉鸡的负面影响
[94]
维生素E 肉鸡 提高胸肉产量和胴体百分比,增加肠道绒毛高度、绒毛
高度与隐窝深度之比和绒毛面积,进而改善肉鸡的肠道形态
[95]
维生素C 提高鸡对疾病的抵抗力、耐热性、食欲和生产性能,
并且通过平滑调节氧化还原平衡来改善免疫器官的
发育,从而提高免疫器官指数和提高体液免疫力
[96]
辅酶Q10 鹌鹑 增加鹌鹑的体重和饲料转化率,使其具有更好的
生长性能,并且使其胸肌含水能力较强、pH升高、
烹饪损失降低,且在免疫反应方面可以取代维生素E
[97]

4.1 多酚类

具有抗氧化性的多酚类物质可以激活Nrf2,主要有白藜芦醇、茶多酚、槲皮素、黄芩素。多酚类的抗氧化活性包括抑制ROS形成、清除ROS、抑制参与产生ROS的酶表达、上调抗氧化防御能力[98]
葡萄籽和果皮以及浆果中的白藜芦醇(3,5,4'-三羟基-反式-二苯乙烯)是一种多酚植物抗毒素,化学式为C14H12O3,属于二苯乙烯家族(一组由亚甲基桥连接的2个芳香环组成的化合物),是一种非类黄酮多酚物质[99],具有抗氧化、抗炎和抗衰老的生理作用[100]。Xun等[80]研究表明,饲粮中补充白藜芦醇可以激活Nrf2,通过提高仔猪血液中SOD、GSH-Px活性和总抗氧化能力(T-AOC)以及降低MDA含量来降低仔猪腹泻,提高生长性能。Yang等[81]报道,饲粮中添加白藜芦醇可以激活Nrf2/HO-1信号通路,提高鸭的抗氧化能力并有效减轻鸭的肝炎和肝脏损伤,最终显著提高平均日增重。
绿茶、水果和蔬菜中的儿茶素是天然多酚化合物,属于黄烷醇类化合物,是茶多酚类物质的主要成分,主体结构是2-苯基苯并吡喃,其根据碳环的不同类型分为4类:表儿茶素(epicatechin,EC)、表没食子儿茶素(epigallocatechin,EGC)、表儿茶素没食子酸酯(epicatechin gallate,ECG)和表没食子儿茶素没食子酸酯(epigallocatechin gallate,EGCG)[101]。Luo等[82]研究表明,饲喂热应激肉鸡EGCG可以增强其抗氧化性能,减轻热应激引起的氧化损伤,提高生长性能。Zhao等[83]研究指出,EGCG通过提高肉鸡肌肉抗氧化能力减少热应激对肝脏和空肠中Nrf2表达的损害,进而改善肉鸡的肉质和肌肉氧化还原平衡。
浆果、坚果、洛瓦奇、苹果、葡萄、洋葱中大量存在的槲皮素[102]是一种多酚化合物,属于类黄酮的亚类(黄酮醇)之一,有15个碳原子和2个由3碳桥连接的芳环[103]。Abdel-Latif等[84]研究发现,饲粮中补充槲皮素显著改善了肉鸡肠道菌群环境,改善了肠道形态和提高了肉鸡的生长性能。梅华迪等[85]研究表明,饲粮中添加槲皮素可以调节断奶仔猪机体代谢,促进有益菌增殖,进而改善肠道健康和促进断奶仔猪生长。
草本植物黄芩茎根中的黄芩素(5,6,7-三羟基黄酮)属于类黄酮之一[104]。Ishfaq等[86]研究表明,在鸡饲粮中添加黄芩素可以降低促炎细胞因子的水平和缓解细胞凋亡,其具有优异的抗菌、抗炎、抗癌和抗病毒特性,显著促进了鸡的生长性能。Wang等[87]研究显示,黄芩素和绿原酸通过改善肠道微生物的组成来减轻蛋鸡的肠道炎症和屏障功能障碍,进而提高蛋鸡的生产性能。Park等[88]研究表明,黄芩提取物可以增加肉鸡的体重和饲料转化率,从而改善其生长性能和营养物质消化率。

4.2 天然色素类

天然色素含大量的酚羟基,因此具有高效的羟基自由基和过氧自由基清除能力,并且还具有强还原性,是极具潜力的天然油脂抗氧化剂,其抗氧化能力是维生素C、维生素E的数倍。常见的天然色素有β-胡萝卜素、番茄红素、虾青素、叶黄素等。
从绿叶的蔬菜和橙黄色的果蔬中提取的叶黄素[105](3’3-二羟基-α-胡萝卜素)又称植物黄体素,属于天然色素的类胡萝卜素(氧化类胡萝卜素)的氧化形式[106]。人和动物不能自行合成叶黄素,外来食物是唯一的叶黄素摄入来源[107]。Liu等[89]研究表明,在蛋鸡饲粮中添加叶黄素增加了老龄母鸡的产蛋率、生育力和孵化率。Wei等[90]研究指出,叶黄素显著提高了黄羽肉鸡皮肤颜色的黄色评分和胴体色素沉着值,从而改善鸡肉的颜色。
从微藻类和益生菌中提取的虾青素(3,3'-二羟基-β,β'-胡萝卜素-4,4'-二酮)是叶黄素亚类的红橙色脂溶性类胡萝卜素色素,也存在于以浮游植物为食的虾、鲑鱼、螃蟹和小龙虾中[108]。在类胡萝卜素中,与角黄质、叶黄素、玉米黄质和β-胡萝卜素相比,虾青素具有更强的抗氧化特性[109]。Hosseindoust等[91]研究表明,补充虾青素可以增强肉鸡在热应激期间的抗氧化防御系统,改善肉品质、生长性能和免疫能力。Awadh等[92]研究显示,饲粮中添加虾青素可以显著提高肉鸡的平均体重、日增重、累计采食量和显著降低饲料系数,且各添加处理的总死亡率均显著降低。
从番茄、西瓜、葡萄柚中提取的番茄红素又称ψ,ψ-胡萝卜素,具有的长链多不饱和烯烃分子结构使其具有很强的消除自由基能力和抗氧化能力[110]。Sun等[93]研究表明,母猪饲粮中补充番茄红素改善了母猪的胎盘健康和乳成分,增加了窝产仔数、出生重和断奶窝重,提高了母猪的繁殖性能。

4.3 维生素及其衍生物

从菠菜、土豆、花椰菜、番茄、豌豆、甘蓝中提取的α-硫辛酸是一种天然线粒体二硫复合物,是丙酮酸脱氢酶和α-酮戊二酸脱氢酶的重要辅酶。Wasti等[94]研究发现,膳食α-硫辛酸补充剂提高了肉鸡的平均日增重、终末体重、肠道绒毛高度和绒毛高度与隐窝深度之比,同时改善了盲肠中有益菌乳酸杆菌的丰度,有效地减轻了热应激对肉鸡的负面影响。
从果蔬、坚果、柑橘皮和胡桃中提取的维生素E,又称生育酚,其抗氧化功能不仅体现在清除自由基方面,还可以去除形成脂过氧化物的潜在来源,抑制组织膜内围绕着细胞颗粒及红细胞的膜内多不饱和脂肪酸的氧化,能与过氧化物反应将其转变为对细胞无害的物质,维持细胞膜中长链多不饱和脂肪酸的完整性,从而维持其生物活性。Peri c '[95]研究表明,添加维生素E提高了胸肉产量和胴体百分比,增加了肠道绒毛高度和绒毛高度与隐窝深度之比,改善了肉鸡的肠道形态。
从新鲜果蔬中提取的维生素C,又称抗坏血酸,易溶于水,微溶于丙酮,其抗氧化活性主要是通过逐级供给电子而转变成半脱氢维生素C,以达到清除自由基的目的。Sun等[96]研究表明,饲粮中添加维生素C可提高鸡对疾病的抵抗力,并且通过调节氧化还原平衡来改善免疫器官的发育,提高免疫器官指数和机体免疫力。
从烟叶和益生菌中提取的辅酶Q10是一种醌类化合物,通常含量极低,在机体中有氧化型和还原型2种存在形式,并且可以相互转化,但是只有还原型才能发挥抗氧化作用,主要体现在清除自由基、稳定细胞膜和抗细胞凋亡方面。Omidizadeh等[97]研究表明,饲粮中添加辅酶Q10可增加鹌鹑的体重和饲料转化率,使其具有更好的生长性能,并提高鹌鹑的肉品质。

4.4 其他营养素

除从天然植物提取的通路激活剂外,很多微量元素和寡糖也具有良好的抗氧化能力。体内的微量元素硒可以清除自由基充当抗氧化剂,通过硒代半胱氨酸和硒蛋白的形式在氧化还原平衡调节中发挥重要作用,参与慢性炎症疾病的发病机制和干预[111]。刘磊[112]研究发现,酵母硒提高了断奶仔猪抗氧化信号相关分子Nrf2和HO-1的表达水平,并显著提高血清、胸腺和肝脏中GSH-Px、CAT和SOD活性,缓解氧化应激对断奶仔猪造成的生长性能下降和肠道屏障氧化损伤。李世印[113]研究发现,饲粮中添加硒代蛋氨酸可提高育肥猪的抗氧化能力,促进器官发育,改善肉品质。郭洁平[114]研究发现,羟基蛋氨酸锌通过提高仔猪体内抗氧化酶的活性,维护肠道屏障功能,进而维护氧化应激仔猪肠道的正常生理功能。魏琳琳等[115]研究发现,饲粮中添加壳寡糖能够通过上调肉鸡胸肌中HO-1的mRNA表达量,提高胸肌的抗氧化性能,并提高肉鸡的平均日增重和降低耗料增重比,同时改善肉品质。王中成[116]研究发现,在肉仔鸡饲粮中添加果胶寡糖螯合锌通过提高机体抗氧化功能、锌营养状态、肠道健康和营养物质消化利用率,提高肉仔鸡的生长性能。

5 小结与展望

本文对Keap1-Nrf2-ARE信号通路各部分的基本分子结构进行了详细阐述,同时对Keap1-Nrf2-ARE信号通路在机体氧化应激反应中的调控机制及其在机体生理上的功能作用进行了分析,对Keap1-Nrf2-ARE信号通路的激活剂进行了分类总结,并概述了其在畜禽生产中的研究案例和试验数据,旨在为今后的氧化应激机制研究及抗氧化活性产品开发提供参考。
随着对Keap1-Nrf2-ARE信号通路调控机制的深入研究,发现越来越多的植物提取物和益生菌在Keap1-Nrf2-ARE信号通路的调节中发挥着重要作用。当前,虽有大量研究证明多种植物提取物和益生菌能够作为通路激活剂激活Keap1-Nrf2-ARE信号通路,却很少有研究阐述说明通路激活剂的调节机制,很少有研究将Keap1-Nrf2-ARE信号通路的激活与畜禽生产性能、肉品质和肠道菌群之间的变化阐述清楚,这些将会是今后我们在研究中需要不断深入探讨的方向。根据Keap1-Nrf2-ARE信号通路的调控机制,可以借助高效的体外细胞试验建立功能性筛选模型,筛选出能够激活ARE基因表达抗氧化酶的活性物质——通路激活剂,用于开发非常规饲料原料或新型功能性饲料添加剂。通路激活剂也有相反作用的实例,有研究发现,高剂量的通路激活剂会抑制营养物质吸收率,引起机体毒副作用[116-118]。因此,在饲料行业绿色、高效、安全的发展要求和全面禁抗背景下,新型饲料添加剂产品的研发不仅要提高饲料利用率和养殖效益,更要符合健康、安全、环保的要求。
[1]
李勇, 孔令青, 高洪, 等. 自由基与疾病研究进展[J]. 动物医学进展, 2008, 29(4):85-88.

LI Y, KONG L Q, GAO H, et al. Progress on free radical and diseases[J]. Progress in Veterinary Medicine, 2008, 29(4):85-88. (in Chinese)

[2]
SARNIAK A, LIPIÑSKA J, TYTMAN K, et al. Endogenous mechanisms of reactive oxygen species (ROS) generation[J]. Postepy Higieny i Medycyny Doswiadczalnej (Online), 2016, 70(0):1150-1165.

[3]
MORIS D, SPARTALIS M, SPARTALIS E, et al. The role of reactive oxygen species in the pathophysiology of cardiovascular diseases and the clinical significance of myocardial redox[J]. Annals of Translational Medicine, 2017, 5(16):326.

DOI PMID

[4]
李海鹏. 热应激对肉鸡生长性能、脂肪沉积及肝脏抗氧化性能的影响[D].硕士学位论文. 荆州: 长江大学, 2021.

LI H P. Effects of heat stress on growth performance,fat deposition and liver anti-oxidative capacity in broilers[D].Master’s Thesis. Jingzhou: Yangtz University, 2021. (in Chinese)

[5]
LI Q H, YANG S W, CHEN F, et al. Nutritional strategies to alleviate oxidative stress in sows[J]. Animal Nutrition, 2022, 9:60-73.

DOI PMID

[6]
高阳, 杜鑫, 马雪, 等. 白藜芦醇对Nrf2、NF-κB和Wnt信号通路的调控及其在动物生产中的应用[J]. 中国畜牧兽医, 2023, 50(2):512-518.

DOI

GAO Y, DU X, MA X, et al. Regulation of resveratrol on Nrf2,NF-κB and Wnt signaling pathways and its application in animals production[J]. China Animal Husbandry & Veterinary Medicine, 2023, 50(2):512-518. (in Chinese)

[7]
王淑楠, 董丽, 刘子娟, 等. 竹酢粉对育肥猪机体抗氧化功能和Nrf2-ARE信号通路基因表达的影响[C]// 中国畜牧兽医学会动物营养学分会第十二次动物营养学术研讨会论文集. 北京: 中国农业大学出版社, 2016:192.

WANG S N, DONG L, LIU Z J, et al. Effects of bamboo sora powder on antioxidant Function and Nrf2-ARE signaling pathway gene expression in fattening pigs[C]// Proceedings of the 12th Academic Symposium on Animal Nutrition of the Animal Nutrition Branch of the Chinese Society of Animal Husbandry and Veterinary Medicine. Beijing: China Agricultural University Press, 2016:192. (in Chinese)

[8]
金旭, 吴琼, 李祯, 等. 益生菌与酸化剂联用对肉鸡生长性能、抗氧化能力和肠道健康的影响[J]. 动物营养学报, 2023, 35(12):7759-7773.

DOI

JIN X, WU Q, LI Z, et al. Effects of probiotics combined with acidifiers on growth performance,antioxidant capacity and intestinal health of broilers[J]. Chinese Journal of Animal Nutrition, 2023, 35(12):7759-7773. (in Chinese)

DOI

[9]
王燕飞, 刘璇, 张若男, 等. 复合益生菌对肉鸡肠道免疫、抗氧化与细胞凋亡的影响[J]. 动物营养学报, 2023, 35(5):2916-2928.

DOI

WANG Y F, LIU X, ZHANG R N, et al. Effects of compound probiotics on intestinal immunity,antioxidation and apoptosis of broilers[J]. Chinese Journal of Animal Nutrition, 2023, 35(5):2916-2928. (in Chinese)

[10]
郑旭, 饶志勇, 孟春颜, 等. 饲粮中添加槲皮万寿菊素对肉鸡生长性能、养分表观消化率和抗氧化能力的影响[J]. 动物营养学报, 2022, 34(7):4271-4282.

DOI

ZHENG X, RAO Z Y, MENG C Y, et al. Effects of dietary quercetagetin on growth performance,nutrient apparent digestibility and antioxidant capacity of broilers[J]. Chinese Journal of Animal Nutrition, 2022, 34(7):4271-4282. (in Chinese)

DOI

[11]
SUZUKI T, YAMAMOTO M. Molecular basis of the Keap1-Nrf2 system[J]. Free Radical Biology & Medicine, 2015, 88(Pt B):93-100.

[12]
TU W J, WANG H, LI S, et al. The anti-inflammatory and anti-oxidant mechanisms of the Keap1/Nrf2/ARE signaling pathway in chronic diseases[J]. Aging and Disease, 2019, 10(3):637-651.

DOI

[13]
BELLEZZA I, GIAMBANCO I, MINELLI A, et al. Nrf2-Keap1 signaling in oxidative and reductive stress[J]. Biochimica et Biophysica Acta:Molecular Cell Research, 2018, 1865(5):721-733.

[14]
YU C, XIAO J H. The Keap1-Nrf2 system:a mediator between oxidative stress and aging[J]. Oxidative Medicine and Cellular Longevity, 2021, 2021:6635460.

[15]
KOBAYASHI A, KANG M I, OKAWA H, et al. Oxidative stress sensor Keap1 functions as an adaptor for Cul3-based E3 ligase to regulate proteasomal degradation of Nrf2[J]. Molecular and Cellular Biology, 2004, 24(16):7130-7139.

DOI PMID

[16]
胡流芳, 王迎, 任汝静, 等. Keap1-Nrf2/ARE信号通路的抗氧化应激作用及其调控机制[J]. 国际药学研究杂志, 2016, 43(1):146-152,166.

HU L F, WANG Y, REN R J, et al. Anti-oxidative stress actions and regulation mechanisms of Keap1-Nrf2/ARE signal pathway[J]. Journal of International Pharmaceutical Research, 2016, 43(1):146-152,166. (in Chinese)

[17]
ZHANG D D, LO S C, CROSS J V, et al. Keap1 is a redox-regulated substrate adaptor protein for a Cul3-dependent ubiquitin ligase complex[J]. Molecular and Cellular Biology, 2004, 24(24):10941-10953.

DOI PMID

[18]
ZIPPER L M, MULCAHY R T. The Keap1 BTB/POZ dimerization function is required to sequester Nrf2 in cytoplasm[J]. Journal of Biological Chemistry, 2002, 277(39):36544-36552.

DOI PMID

[19]
ZHANG D D, HANNINK M. Distinct cysteine residues in Keap1 are required for Keap1-dependent ubiquitination of Nrf2 and for stabilization of Nrf2 by chemopreventive agents and oxidative stress[J]. Molecular and Cellular Biology, 2003, 23(22):8137-8151.

DOI PMID

[20]
YAMAMOTO T, SUZUKI T, KOBAYASHI A, et al. Physiological significance of reactive cysteine residues of Keap1 in determining Nrf2 activity[J]. Molecular and Cellular Biology, 2008, 28(8):2758-2770.

DOI PMID

[21]
KOBAYASHI M, ITOH K, SUZUKI T, et al. Identification of the interactive interface and phylogenic conservation of the Nrf2-Keap1 system[J]. Genes to Cells, 2002, 7(8):807-820.

DOI PMID

[22]
TONG K I, PADMANABHAN B, KOBAYASHI A, et al. Different electrostatic potentials define ETGE and DLG motifs as hinge and latch in oxidative stress response[J]. Molecular and Cellular Biology, 2007, 27(21):7511-7521.

DOI PMID

[23]
ROJO DE LA VEGA M, CHAPMAN E, ZHANG D D. NRF2 and the hallmarks of cancer[J]. Cancer Cell, 2018, 34(1):21-43.

DOI PMID

[24]
TONELLI C, CHIO I I C, TUVESON D A. Transcriptional regulation by Nrf2[J]. Antioxidants & Redox Signaling, 2018, 29(17):1727-1745.

[25]
ADELUSI T I, DU L, HAO M, et al. Keap1/Nrf2/ARE signaling unfolds therapeutic targets for redox imbalanced-mediated diseases and diabetic nephropathy[J]. Biomedicine & Pharmacotherapy, 2020, 123:109732.

[26]
HOLMSTRÖM K M, BAIRD L, ZHANG Y, et al. Nrf2 impacts cellular bioenergetics by controlling substrate availability for mitochondrial respiration[J]. Biology Open, 2013, 2(8):761-770.

DOI PMID

[27]
SYKIOTIS G P, BOHMANN D. Stress-activated Cap‘n’collar transcription factors in aging and human disease[J]. Science Signaling, 2010, 3(112):re3.

[28]
KWAK M K, KENSLER T W. Targeting NRF2 signaling for cancer chemoprevention[J]. Toxicology and Applied Pharmacology, 2010, 244(1):66-76.

[29]
HIGGINS L G, KELLEHER M O, EGGLESTON I M, et al. Transcription factor Nrf2 mediates an adaptive response to sulforaphane that protects fibroblasts in vitro against the cytotoxic effects of electrophiles,peroxides and redox-cycling agents[J]. Toxicology and Applied Pharmacology, 2009, 237(3):267-280.

[30]
MCMAHON M, ITOH K, YAMAMOTO M, et al. Keap1-dependent proteasomal degradation of transcription factor Nrf2 contributes to the negative regulation of antioxidant response element-driven gene expression[J]. Journal of Biological Chemistry, 2003, 278(24):21592-21600.

DOI PMID

[31]
KANSANEN E, KUOSMANEN S M, LEINONEN H, et al. The Keap1-Nrf2 pathway:mechanisms of activation and dysregulation in cancer[J]. Redox Biology, 2013, 1(1):45-49.

[32]
KATOH Y, ITOH K, YOSHIDA E, et al. Two domains of Nrf2 cooperatively bind CBP,a CREB binding protein,and synergistically activate transcription[J]. Genes to Cells, 2001, 6(10):857-868.

[33]
ZHANG J Y, OHTA T, MARUYAMA A, et al. BRG1 interacts with Nrf2 to selectively mediate HO-1 induction in response to oxidative stress[J]. Molecular and Cellular Biology, 2006, 26(21):7942-7952.

PMID

[34]
WANG H Y, LIU K H, GENG M, et al. RXRα inhibits the NRF2-ARE signaling pathway through a direct interaction with the Neh7 domain of NRF2[J]. Cancer Research, 2013, 73(10):3097-3108.

DOI PMID

[35]
CHOWDHRY S, ZHANG Y, MCMAHON M, et al. Nrf2 is controlled by two distinct β-TrCP recognition motifs in its Neh6 domain,one of which can be modulated by GSK-3 activity[J]. Oncogene, 2013, 32(32):3765-3781.

[36]
ITOH K, MIMURA J, YAMAMOTO M. Discovery of the negative regulator of Nrf2,Keap1:a historical overview[J]. Antioxidants & Redox Signaling, 2010, 13(11):1665-1678.

[37]
MOTOHASHI H, KATSUOKA F, ENGEL J D, et al. Small Maf proteins serve as transcriptional cofactors for keratinocyte differentiation in the Keap1-Nrf2 regulatory pathway[J]. Proceedings of the National Academy of Sciences of the United States of America, 2004, 101(17):6379-6384.

PMID

[38]
NIOI P, NGUYEN T, SHERRATT P J, et al. The carboxy-terminal Neh3 domain of Nrf2 is required for transcriptional activation[J]. Molecular and Cellular Biology, 2005, 25(24):10895-10906.

DOI PMID

[39]
RAMOS-GOMEZ M, KWAK M K, DOLAN P M, et al. Sensitivity to carcinogenesis is increased and chemoprotective efficacy of enzyme inducers is lost in Nrf2 transcription factor-deficient mice[J]. Proceedings of the National Academy of Sciences of the United States of America, 2001, 98(6):3410-3415.

[40]
RAMOS-GOMEZ M, DOLAN P M, ITOH K, et al. Interactive effects of Nrf2 genotype and oltipraz on benzo[a]pyrene-DNA adducts and tumor yield in mice[J]. Carcinogenesis, 2003, 24(3):461-467.

[41]
KWAK M K, ITOH K, YAMAMOTO M, et al. Role of transcription factor Nrf2 in the induction of hepatic phase 2 and antioxidative enzymes in vivo by the cancer chemoprotective agent,3H-1,2-dimethiole-3-thione[J]. Molecular Medicine, 2001, 7(2):135-145.

[42]
RUSHMORE T H, PICKETT C B. Transcriptional regulation of the rat glutathione S-transferase Ya subunit gene.Characterization of a xenobiotic-responsive element controlling inducible expression by phenolic antioxidants[J]. The Journal of Biological Chemistry, 1990, 265(24):14648-14653.

[43]
FRILING R S, BENSIMON A, TICHAUER Y, et al. Xenobiotic-inducible expression of murine glutathione S-transferase Ya subunit gene is controlled by an electrophile-responsive element[J]. Proceedings of the National Academy of Sciences of the United States of America, 1990, 87(16):6258-6262.

DOI PMID

[44]
XU C J, LI C Y T, KONG A N T. Induction of phase Ⅰ,Ⅱ and Ⅲ drug metabolism/transport by xenobiotics[J]. Archives of Pharmacal Research, 2005, 28(3):249-268.

[45]
MIAO W M, HU L G, SCRIVENS P J, et al. Transcriptional regulation of NF-E2 p45-related factor (NRF2) expression by the aryl hydrocarbon receptor-xenobiotic response element signaling pathway:direct cross-talk between phase Ⅰ and Ⅱ drug-metabolizing enzymes[J]. The Journal of Biological Chemistry, 2005, 280(21):20340-20348.

[46]
TELAKOWSKI-HOPKINS C A, KING R G, PICKETT C B. Glutathione S-transferase Ya subunit gene:identification of regulatory elements required for basal level and inducible expression[J]. Proceedings of the National Academy of Sciences of the United States of America, 1988, 85(4):1000-1004.

[47]
RAGHUNATH A, SUNDARRAJ K, NAGARAJAN R, et al. Antioxidant response elements:discovery,classes,regulation and potential applications[J]. Redox Biology, 2018, 17:297-314.

[48]
HE B, CHEN D Y, ZHANG X C, et al. Oxidative stress and ginsenosides:an update on the molecular mechanisms[J]. Oxidative Medicine and Cellular Longevity, 2022, 2022:9299574.

[49]
WU S J, LU H, BAI Y H. Nrf2 in cancers:a double-edged sword[J]. Cancer Medicine, 2019, 8(5):2252-2267.

[50]
IZUMI Y, TATSUMOTO A, HORIUCHI N, et al. TPNA10168,an Nrf-2 activator,attenuates inflammatory responses independently of Nrf2 in microglial BV-2 cells:involvement of the extracellular-signal-regulated kinase pathway[J]. Journal of Pharmacological Sciences, 2022, 149(1):1-10.

[51]
熊款款, 谭磊, 王爱兵, 等. Keap 1-Nrf2/ARE信号通路抗氧化机制及抗氧化剂的研究进展[J]. 动物医学进展, 2021, 42(4):89-94.

XIONG K K, TAN L, WANG A B, et al. Progress on anti-oxidation mechanisms and antioxidants of the Keap1-Nrf2/ARE signaling pathway[J]. Progress in Veterinary Medicine, 2019, 42(4):89-94. (in Chinese)

[52]
李慧, 杨林. Nrf2抗氧化的分子调控机制[J]. 生物信息学, 2018, 16(1):1-6.

LI H, YANG L. Molecular regulatory mechanism of Nrf2 antioxidant[J]. Chinese Journal of Bioinformatics, 2018, 16(1):1-6. (in Chinese)

[53]
XU Z Q, CHU M. Advances in immunosuppressive agents based on signal pathway[J]. Frontiers in Pharmacology, 2022, 13:917162.

[54]
丁子惠, 袁月, 宋双, 等. 破血化瘀填精补髓中药汤剂对核因子E2相关因子2基因敲除脑出血小鼠氧化应激的影响[J]. 中华老年心脑血管病杂志, 2022, 24(5):536-540.

DING Z H, YUAN Y, SONG S, et al. Effect of blood stasis removing,essence replenishing decoction on oxidative stress in Nrf2 gene knocked-out intracerebral hemorrhage mice[J]. Chinese Journal of Geriatric Heart Brain and Vessel Diseases, 2022, 24(5):536-540. (in Chinese)

[55]
HUANG H C, NGUYEN T, PICKETT C B. Phosphorylation of Nrf2 at Ser-40 by protein kinase C regulates antioxidant response element-mediated transcription[J]. Journal of Biological Chemistry, 2002, 277(45):42769-42774.

DOI PMID

[56]
HAYES J D, CHOWDHRY S, DINKOVA-KOSTOVA A T, et al. Dual regulation of transcription factor Nrf2 by Keap1 and by the combined actions of β-TrCP and GSK-3[J]. Biochemical Society Transactions, 2015, 43(4):611-620.

DOI PMID

[57]
KANG K W, CHO M K, LEE C H, et al. Activation of phosphatidylinositol 3-kinase and Akt by tert-butylhydroquinone is responsible for antioxidant response element-mediated rGSTA2 induction in H4IIE cells[J]. Molecular Pharmacology, 2001, 59(5):1147-1156.

DOI PMID

[58]
JOO M S, KIM W D, LEE K Y, et al. AMPK facilitates nuclear accumulation of Nrf2 by phosphorylating at serine 550[J]. Molecular and Cellular Biology, 2016, 36(14):1931-1942.

DOI PMID

[59]
WU T D, ZHAO F, GAO B X, et al. Hrd1 suppresses Nrf2-mediated cellular protection during liver cirrhosis[J]. Genes & Development, 2014, 28(7):708-722.

[60]
WEN C Y, ZHANG H, GUO Q P, et al. Engineered Bacillus subtilis alleviates intestinal oxidative injury through Nrf2-Keap1 pathway in enterotoxigenic Escherichia coli (ETEC) K88-infected piglet[J]. Journal of Zhejiang University:Science B, 2023, 24(6):496-509.

[61]
王琳燚, 徐彬, 王丁, 等. 金银花提取物对肉鸡生产性能、屠宰性能、肉品质和抗氧化性能的影响[J]. 河南农业科学, 2022, 51(10):134-141.

WANG L Y, XU B, WANG D, et al. Effects of extract from Lonicera japonica Thunb. on the production performance,slaughter characters,meat quality and antioxidant capacity of broilers[J]. Journal of Henan Agricultural Sciences, 2022, 51(10):134-141. (in Chinese)

[62]
AHMED S M U, LUO L, NAMANI A, et al. Nrf2 signaling pathway:pivotal roles in inflammation[J]. Biochimica et Biophysica Acta:Molecular Basis of Disease, 2017, 1863(2):585-597.

[63]
KOBAYASHI E H, SUZUKI T, FUNAYAMA R, et al. Nrf2 suppresses macrophage inflammatory response by blocking proinflammatory cytokine transcription[J]. Nature Communications, 2016, 7:11624.

DOI PMID

[64]
HUANG Y, LI W J, SU Z Y, et al. The complexity of the Nrf2 pathway:beyond the antioxidant response[J]. The Journal of Nutritional Biochemistry, 2015, 26(12):1401-1413.

[65]
WANG S L, LI C, ZHANG C S, et al. Effects of Sihuang Zhili granules on the diarrhea symptoms,immunity,and antioxidant capacity of poultry challenged with lipopolysaccharide (LPS)[J]. Antioxidants, 2023, 12(7):1372.

[66]
VÁNYOLÓS A, MUSZYÑSKA B, CHULUUNBAATAR B, et al. Extracts and steroids from the edible mushroom Hypholoma lateritium exhibit anti-inflammatory properties by inhibition of COX-2 and activation of Nrf2[J]. Chemistry & Biodiversity, 2020, 17(9):e2000391.

[67]
WU K C, LIU J, KLAASSEN C D. Role of Nrf2 in preventing ethanol-induced oxidative stress and lipid accumulation[J]. Toxicology and Applied Pharmacology, 2012, 262(3):321-329.

DOI PMID

[68]
谭斅. 木犀草素对鹌鹑机体影响及其缓解无机汞致肝肾损伤作用[D]. 博士学位论文. 哈尔滨: 东北农业大学, 2020.

TAN X. Effects of luteolin on quails and its mitigation of liver and kidney injury induced by inorganic mercury[D]. Ph.D.Thesis.Harbin:Northeast Agricultural University, 2020. (in Chinese)

[69]
陈诺, 金华, 呼琴, 等. 清肾颗粒对腺嘌呤致肾纤维化大鼠Nrf2/ARE信号通路及氧化应激的干预作用[J]. 中医药临床杂志, 2023, 35(5):976-982.

CHEN N, JIN H, HU Q, et al. Effect of qingshen granule on Nrf2/ARE in rats with adenine induced renal fibrosis signal pathway and the intervention of oxidative stress[J]. Clinical Journal of Traditional Chinese Medicine, 2023, 35(5):976-982. (in Chinese)

[70]
刘运华, 张新雪, 高坤, 等. 基于Keap1/Nrf2/HO-1信号转导通路探讨糖肾宁防治糖尿病肾病的作用机制[J]. 中华中医药杂志, 2023, 38(5):2409-2417.

LIU Y H, ZHANG X X, GAO K, et al. Discussion on the mechanism of Tangshenning in the prevention and treatment of diabetic kidney disease based on Keap1/Nrf2/HO-1 signaling pathway[J]. China Journal of Traditional Chinese Medicine and Pharmacy, 2019, 38(5):2409-2417. (in Chinese)

[71]
HAYES J D, DINKOVA-KOSTOVA A T. The Nrf2 regulatory network provides an interface between redox and intermediary metabolism[J]. Trends in Biochemical Sciences, 2014, 39(4):199-218.

DOI PMID

[72]
DENG L L. Astragaloside IV as potential antioxidant against diabetic ketoacidosis in juvenile mice through activating JNK/Nrf2 signaling pathway[J]. Archives of Medical Research, 2020, 51(7):654-663.

[73]
孙梦雪, 韩雪, 杨玉辉, 等. 虫草发酵菌丝体对胰岛素抵抗大鼠氧化应激的缓解作用[J]. 天然产物研究与开发, 2019, 31(7):1278-1284.

SUN M X, HAN X, YANG Y H, et al. Cordyceps fermentation mycelium attenuates oxidative stress in rats with insulin resistance[J]. Natural Product Research and Development, 2019, 31(7):1278-1284. (in Chinese)

DOI

[74]
DINKOVA-KOSTOVA A T, HOLTZCLAW W D, COLE R N, et al. Direct evidence that sulfhydryl groups of Keap1 are the sensors regulating induction of phase 2 enzymes that protect against carcinogens and oxidants[J]. Proceedings of the National Academy of Sciences of the United States of America, 2002, 99(18):11908-11913.

[75]
MARZIONI D, MAZZUCCHELLI R, FANTONE S, et al. NRF2 modulation in TRAMP mice: an in vivo model of prostate cancer[J]. Molecular Biology Reports, 2023, 50(1):873-881.

[76]
SHAHCHERAGHI S H, SALEMI F, SMALL S, et al. Resveratrol regulates inflammation and improves oxidative stress via Nrf2 signaling pathway:therapeutic and biotechnological prospects[J]. Phytotherapy Research, 2023, 37(4):1590-1605.

[77]
黄婷芸, 黄南渠, 保玉心. Keap1/Nrf2/ARE信号通路及激活剂在帕金森病研究中的进展[J]. 遵义医科大学学报, 2023, 46(5):520-528,536.

HUANG T Y, HUANG N Q, BAO Y X. Keap1-Nrf2-ARE signaling pathway and activators in Parkinson’s disease:a review[J]. Journal of Zunyi Medical University, 2023, 46(5):520-528,536. (in Chinese)

[78]
姚娟, 吴平安, 李芸, 等. Keap1-Nrf2-ARE信号通路及其激活剂的研究进展[J]. 中国药理学通报, 2019, 35(10):1342-1346.

YAO J, WU P A, LI Y, et al. Research progress of small molecule activators in Keap1-Nrf2-ARE signaling pathway[J]. Chinese Pharmacological Bulletin, 2019, 35(10):1342-1346. (in Chinese)

[79]
QIN S, HOU D X. The biofunctions of phytochemicals and their applications in farm animals: the Nrf2/Keap1 system as a target[J]. Engineering, 2017, 3(5):738-752.

[80]
XUN W J, FU Q Y, HOU G Y, et al. Protective effects of dietary resveratrol supplementation against oxidative stress in diquat-challenged piglets[J]. Italian Journal of Animal Science, 2020, 19(1):1523-1532.

[81]
YANG H, WANG Y J, LIU M R, et al. Effects of dietary resveratrol supplementation on growth performance and anti-inflammatory ability in ducks (Anas platyrhynchos) through the Nrf2/HO-1 and TLR4/NF-κB signaling pathways[J]. Animals, 2021, 11(12):3588.

[82]
LUO J X, SONG J, LIU L Z, et al. Effect of epigallocatechin gallate on growth performance and serum biochemical metabolites in heat-stressed broilers[J]. Poultry Science, 2018, 97(2):599-606.

DOI PMID

[83]
ZHAO F, WANG X C, LI Y, et al. Effects of dietary supplementation with epigallocatechin gallate on meat quality and muscle antioxidant capacity of broilers subjected to acute heat stress[J]. Animals, 2021, 11(11):3296.

[84]
ABDEL-LATIF M A, ELBESTAWY A R, EL-FAR A H, et al. Quercetin dietary supplementation advances growth performance,gut microbiota,and intestinal mRNA expression genes in broiler chickens[J]. Animals, 2021, 11(8):2302.

[85]
梅华迪, 李袁飞, 田琦, 等. 槲皮素对断奶仔猪生长性能、营养物质表观消化率、血清生化指标、粪便微生物及其代谢产物的影响[J]. 动物营养学报, 2022, 34(5):2884-2895.

DOI

MEI H D, LI Y F, TIAN Q, et al. Effects of quercetin on growth performance,nutrient apparent digestibility,serum biochemical indices,fecal microorganisms and their metabolites of weaned piglets[J]. Chinese Journal of Animal Nutrition, 2022, 34(5):2884-2895. (in Chinese)

[86]
ISHFAQ M, ZHANG W, LIU Y H, et al. Baicalin attenuated Mycoplasma gallisepticum-induced immune impairment in chicken bursa of fabricius through modulation of autophagy and inhibited inflammation and apoptosis[J]. Journal of the Science of Food and Agriculture, 2021, 101(3):880-890.

[87]
WANG W W, JIA H J, ZHANG H J, et al. Supplemental plant extracts from Flos lonicerae in combination with Baikal skullcap attenuate intestinal disruption and modulate gut microbiota in laying hens challenged by Salmonella pullorum[J]. Frontiers in Microbiology, 2019, 10:1681.

[88]
PARK J H, PI S H, KIM I H. Growth performance,blood profile,nutrient digestibility and meat quality of broilers fed on diets supplemented with Scutellaria baicalensis extract[J]. European Poultry Science, 2016, 80:1-10.

[89]
LIU N, JI X, SONG Z, et al. Effect of dietary lutein on the egg production,fertility,and oxidative injury indexes of aged hens[J]. Animal Bioscience, 2023, 36(8):1221-1227.

[90]
WEI Y, QIN K, QIN X, et al. Effects of different types of xanthophyll extracted from marigold on pigmentation of yellow-feathered chickens[J]. Animal Bioscience, 2023, 36(12):1853-1859.

[91]
HOSSEINDOUST A, OH S M, KO H S, et al. Muscle antioxidant activity and meat quality are altered by supplementation of astaxanthin in broilers exposed to high temperature[J]. Antioxidants, 2020, 9(11):1032.

[92]
AWADH I A J, ZANGANA B S R. The effect of adding different levels of astaxanthin on the productive performance of broilers chicken reared under high environmental temperatures[J]. Plant Archives, 2020, 20(2):4069-4075.

[93]
SUN S S, MENG Q W, BAI Y S, et al. Lycopene improves maternal reproductive performance by modulating milk composition and placental antioxidative and immune status[J]. Food & Function, 2021, 12(24):12448-12467.

[94]
WASTI S, SAH N, LEE C N, et al. Dietary supplementation of alpha-lipoic acid mitigates the negative effects of heat stress in broilers[J]. PLoS One, 2021, 16(7):e0254936.

[95]
PERIĆ L, ŽIKIĆ D, STOJĆIĆ M D, et al. Effect of chestnut tannins and vitamin E supplementation to linseed oil-enriched diets on growth performance,meat quality,and intestinal morphology of broiler chickens[J]. Agriculture,2022,12(11):1772.

[96]
SUN S A, LI B, WU M M, et al. Effect of dietary supplemental vitamin C and betaine on the growth performance,humoral immunity,immune organ index,and antioxidant status of broilers under heat stress[J]. Tropical Animal Health and Production, 2023, 55(2):96.

[97]
OMIDIZADEH M, KHEIRI F, FAGHANI M. Coenzyme Q 10 in quail nutrition:effects on growth performance,meat quality,and myostatin gene expression[J]. Livestock Science, 2021, 252:104682.

[98]
CARDOZO L F M F, PEDRUZZI L M, STENVINKEL P, et al. Nutritional strategies to modulate inflammation and oxidative stress pathways via activation of the master antioxidant switch Nrf2[J]. Biochimie, 2013, 95(8):1525-1533.

DOI PMID

[99]
BOLA C, BARTLETT H, EPERJESI F. Resveratrol and the eye:activity and molecular mechanisms[J]. Graefe’s Archive for Clinical and Experimental Ophthalmology, 2014, 252(5):699-713.

[100]
ZHANG J, PAVEK P, KAMARAJ R, et al. Dietary phytochemicals as modulators of human pregnane X receptor[J]. Critical Reviews in Food Science and Nutrition, 2023, 63(19):3279-3301.

[101]
BRAICU C, LADOMERY M R, CHEDEA V S, et al. The relationship between the structure and biological actions of green tea catechins[J]. Food Chemistry, 2013, 141(3):3282-3289.

DOI PMID

[102]
ANAND DAVID A V, ARULMOLI R, PARASURAMAN S. Overviews of biological importance of quercetin:a bioactive flavonoid[J]. Pharmacognosy Reviews, 2016, 10(20):84-89.

[103]
LIN J, ZHOU W B. Role of quercetin in the physicochemical properties,antioxidant and antiglycation activities of bread[J]. Journal of Functional Foods, 2018, 40:299-306.

[104]
BIE B B, SUN J, GUO Y, et al. Baicalein:a review of its anti-cancer effects and mechanisms in hepatocellular carcinoma[J]. Biomedicine & Pharmacotherapy, 2017, 93:1285-1291.

[105]
贾梅. 叶黄素不仅保护视力,更影响大脑认知功能[J]. 中国妇幼健康研究, 2018, 29(6):801.

JIA M. Lutein not only protects vision, but also affects brain cognitive function[J]. Chinese Journal of Woman and Child Health Research, 2018, 29(6):801. (in Chinese)

[106]
陈城, 程曦, 黄丛林, 等. 叶黄素的提取方法和功能研究进展[J]. 河北林业科技, 2016(3):71-75.

CHEN C, CHENG X, HUANG C L, et al. Research progresses on extraction methods and functions of lutein[J]. The Journal of Hebei Forestry Science and Technology, 2016(3):71-75. (in Chinese)

[107]
马少杰. 婴幼儿配方奶粉中叶黄素的稳定性研究[D].硕士学位论文. 哈尔滨: 东北农业大学, 2018.

MA S J. Study on the stability of lutein in infant formula milk powder[D].Master’s Thesis.Harbin:Northeast Agricultural University, 2018. (in Chinese)

[108]
FAKHRI S, ABBASZADEH F, DARGAHI L, et al. Astaxanthin:a mechanistic review on its biological activities and health benefits[J]. Pharmacological Research, 2018, 136:1-20.

[109]
SEABRA L M J, PEDROSA L F C. Astaxanthin:structural and functional aspects[J]. Revista de Nutrição, 2010, 23(6):1041-1050.

[110]
陈锦瑶, 张立实. 番茄红素的生物学作用及应用研究进展[J]. 卫生研究, 2013, 42(2):336-342.

CHEN J Y, ZHANG L S. Research progress on biological effects and application of lycopene[J]. Journal of Hygiene Research, 2013, 42(2):336-342. (in Chinese)

[111]
HILAL T, KILLAM B Y, GROZDANOVIĆ M, et al. Structure of the mammalian ribosome as it decodes the selenocysteine UGA codon[J]. Science, 2022, 376(6599):1338-1343.

DOI PMID

[112]
刘磊. 酵母硒对氧化应激诱导断奶仔猪生长性能、免疫功能及肠道健康的影响[D].硕士学位论文. 成都: 四川农业大学, 2021.

LIU L. Effects of selenium yeast on growth performance,immune function and intestinal health of weaned piglets exposed to oxidative stress[D].Master’s Thesis. Chengdu: Sichuan Agricultural University, 2021. (in Chinese)

[113]
李世印. 不同硒源对断奶小鼠和育肥猪生长性能和抗氧化的影响[D].硕士学位论文. 泰安: 山东农业大学, 2021.

LI S Y. Effects of different selenium sources on growth performance and antioxidant capacity of weaned mice and finishing pigs[D].Master’s Thesis. Tai’an: Shandong Agricultural University, 2021. (in Chinese)

[114]
郭洁平. 羟基蛋氨酸锌对仔猪氧化应激的影响及相关机制[D]. 博士学位论文. 长沙: 湖南农业大学, 2020.

GUO J P. Effects of dietary supplementations of Zn from different sources on antioxidant capacity of weaned piglets[D]. Ph.D.Thesis. Changsha: Hunan Agricultural University, 2020. (in Chinese)

[115]
魏琳琳, 兰瑞霞, 王语晨, 等. 壳寡糖对肉鸡生长性能、屠宰性能、胸肌肉品质及氧化稳定性的影响[J]. 中国畜牧杂志, 2024, 60(1):307-313.

WEI L L, LAN R X, WANG Y C, et al. Effects of chito-oligosaccharides on growth performance,slaughter performance,breast muscle quality and oxidation stability of broilers[J]. Chinese Journal of Animal Science, 2024, 60(1):307-313. (in Chinese)

[116]
王中成. 果胶寡糖螯合锌对肉仔鸡生长调控机制的研究[D]. 博士学位论文. 北京: 中国农业科学院, 2019.

WANG Z C. Study on the regulatory mechanism of dietary zinc pectin oligosaccharides chelate on growth performance in broiler chickens[D]. Ph.D.Thesis. Beijing: Chinese Academy of Agricultural Sciences, 2019. (in Chinese)

[117]
INOUE H, AKIYAMA S, MAEDA-YAMAMOTO M, et al. High-dose green tea polyphenols induce nephrotoxicity in dextran sulfate sodium-induced colitis mice by down-regulation of antioxidant enzymes and heat-shock protein expressions[J]. Cell Stress & Chaperones, 2011, 16(6):653-662.

[118]
YILMAZER-MUSA M, GRIFFITH A M, MICHELS A J, et al. Grape seed and tea extracts and catechin 3-gallates are potent inhibitors of α-amylase and α-glucosidase activity[J]. Journal of Agricultural and Food Chemistry, 2012, 60(36):8924-8929.

文章导航

/