综述

牛磺酸的生物学功能及其在动物生产中的应用研究进展

  • 刘新宇 , 1, 2 ,
  • 栾嘉明 1, 2 ,
  • 冯鑫 1, 2 ,
  • 耿春银 , 1, 2, *
展开
  • 1 延边大学农学院,延吉 133000
  • 2 延边大学,东北寒区肉牛科技创新教育部工程研究中心,延吉 133002
*耿春银,教授,博士生导师,E-mail:

刘新宇(2000—),男,吉林长岭人,博士研究生,研究方向为反刍动物营养。E-mail:

Copy editor: 菅景颖

收稿日期: 2025-04-20

  网络出版日期: 2025-11-14

基金资助

国家自然科学基金项目(32060763)

国家自然科学基金项目(31660669)

吉林省科技发展项目(YDZJ202203CGZH042)

吉林省科技发展项目(20220202048NC)

吉林省教育厅科学研究项目(JJKH20220542KJ)

Research Progress on Biological Functions of Taurine and Its Application in Animal Production

  • LIU Xinyu , 1, 2 ,
  • LUAN Jiaming 1, 2 ,
  • FENG Xin 1, 2 ,
  • GENG Chunyin , 1, 2, *
Expand
  • 1 College of Agriculture, Yanbian University, Yanji 133000, China
  • 2 Engineering Research Center of North-East Cold Region Beef Cattle Science and Technology Innovation, Ministry of Education, Yanbian University, Yanji 133002, China
*professor, E-mail:

Received date: 2025-04-20

  Online published: 2025-11-14

摘要

牛磺酸是一种在哺乳动物组织中含量很高的游离氨基酸,具有消炎、抗氧化等广泛的生物学功能。牛磺酸作为饲料添加剂已逐步被验证具有改善畜禽生产性能、肠道健康以及产品品质等作用。尽管如此,目前牛磺酸在动物生产中的应用潜力未得到充分开发,尤其在调控反刍动物瘤胃微生物以及与其他益生素协同使用的效果与影响机制还尚不明确。本文综述了牛磺酸的生物学功能、作用机制以及其在动物生产中的应用进展,并对影响牛磺酸应用效果的因素进行了总结,旨在为牛磺酸的高效利用提供参考。

本文引用格式

刘新宇 , 栾嘉明 , 冯鑫 , 耿春银 . 牛磺酸的生物学功能及其在动物生产中的应用研究进展[J]. 动物营养学报, 2025 , 37(11) : 7285 -7297 . DOI: 10.12418/CJAN2025.593

Abstract

Taurine is a free amino acid with a high content in mammalian tissues and has a wide range of biological functions such as anti-inflammatory and antioxidant properties. As a feed additive, taurine has been progressively demonstrated to improve livestock and poultry production performance, enhance intestinal health, and upgrade product quality. However, its full potential in animal production remains underexplored, particularly regarding its modulation of rumen microbiota in ruminants and synergistic interactions with probiotics; the underlying mechanisms of these effects require further investigation. This paper reviewed the biological functions and mechanisms of action of taurine, summarized its advancements in animal production applications, and synthesized factors influencing its efficacy, aiming to provide references for the efficient utilization of taurine.

牛磺酸是一种不参与蛋白质合成的含硫氨基酸,最早由Tiedemann和Gmelin于1827年从牛胆汁中成功分离,广泛分布于动物组织和多种食物中。研究表明,在心脏、视网膜、中枢神经系统及骨骼肌等代谢活性高的组织中,牛磺酸呈现显著富集现象[1]。牛磺酸在肝脏中由蛋氨酸或半胱氨酸合成,其在维持细胞稳态和代谢平衡中发挥关键作用,新生儿和幼儿无法像成年人那样合成牛磺酸或部分组织在特定生理状态下需依赖外源补充以满足其生长发育和生理功能的需求,所以牛磺酸也被称为条件性必需氨基酸[2-3]。在畜牧生产领域中,牛磺酸作为一种功能性饲料添加剂已获得广泛关注,已有研究证实其具有抗氧化[4]、抗炎症[5]、调节脂质代谢稳态[6]以及改善肠道微生态平衡[7]等作用,可使动物生长性能提升、饲料效率改善、肠道屏障功能完善及产品品质优化,同时能有效缓解各类应激反应。基于此,本文综述了牛磺酸的生理学功能、作用机制以及影响其应用效果的因素,为其在动物生产中的应用提供参考。

1 牛磺酸的理化性质
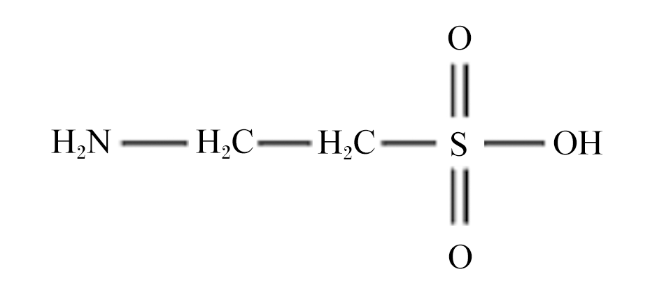
牛磺酸化学名称为2-氨基乙磺酸,是一种含硫的有机化合物,分子式为C2H7NO3S,常温下为白色结晶或结晶性粉末,熔点为300 ℃,易溶于水,不溶于有机溶剂[8],化学性质稳定,其化学结构式如图1所示。
图1 牛磺酸的化学结构式

Fig.1 Chemical structural formula of taurine

2 牛磺酸的生物学功能及其作用机制

2.1 抗氧化能力

活性氧(reactive oxygen species,ROS)的过量产生可导致氧化还原稳态失衡,进而引发蛋白质、脂质及DNA生物大分子的氧化损伤,最终造成细胞功能障碍[9]。牛磺酸具有抗氧化作用,可有效缓解体内氧化应激过程。研究表明,在赭曲霉毒素A诱导的PK-15细胞模型中,牛磺酸可显著降低细胞内ROS含量,下调环氧合酶-2(cyclooxygenase-2,COX-2)和诱导型一氧化氮合酶(iNOS)的mRNA表达水平,同时上调多种抗氧化基因的表达,从而减轻细胞焦亡和细胞毒性[10]。核因子E2相关因子2(nuclear factor erythroid 2 related factor 2,Nrf2)是调控抗氧化应激相关通路的关键转录因子。在生理条件下,Nrf2由细胞质中的Kelch样ECH相关蛋白1(Kelch like ECH associated protein 1,Keap1)锚定[11],氧化应激时,两者解偶联,然后转运到细胞核中,与核内抗氧化应答元件(antioxidant responsive element,ARE)结合,通过诱导抗氧化基因的转录,从而保护细胞免受氧化应激损伤[12-13]。研究报道,牛磺酸可抑制2型糖尿病大鼠氧化应激,反映在改善较低的超氧化物歧化酶(superoxide dismutase,SOD)活性和较高的丙二醛(mmalondialdehyde,MDA)含量上,同时下调Keap1的mRNA表达水平以及上调Nrf2和血红素加氧酶-1(heme oxygenase-1,HO-1)的mRNA表达水平,验证了牛磺酸可通过对Keap1-Nrf2信号传导的调节实现缓解糖尿病大鼠氧化应激[4]。此外,牛磺酸还可通过激活Nrf2信号通路及其下游抗氧化酶来逆转黄曲霉毒素B1、过氧化氢(H2O2)诱导线粒体受氧化应激的影响,从而缓解细胞损伤[14-15]。在胰岛素抵抗模型中,牛磺酸可通过激活磷脂酰肌醇3激酶(phosphatidylinositol 3 kinase,PI3K)/蛋白激酶B(protein kinase B,Akt)信号通路,显著降低ROS荧光强度和MDA含量,同时提高SOD活性和谷胱甘肽(glutathione,GSH)含量,从而改善糖尿病大鼠的氧化应激状态[16]。此外,在采用牛磺酸干预H2O2诱导的成骨细胞氧化应激模型的试验研究中进一步发现,牛磺酸能够通过激活Wnt/β-连环蛋白(β-catenin)信号通路,调控细胞外信号调节激酶(extracellular signal-regulated kinase,ERK)的磷酸化水平,进而显著增强细胞的抗氧化防御能力[17]
综上可知,牛磺酸可通过多途径、多靶点来发挥抗氧化作用,其抗氧化作用机制复杂,可调控Keap1-Nrf2、PI3K/Akt、Wnt/β-catenin等信号通路来调节抗氧化酶系统,改善机体氧化应激反应。

2.2 抗炎能力

炎症反应作为机体应对感染和组织损伤的重要防御机制,其核心功能在于修复受损组织并恢复内环境稳态。适度的急性炎症反应可有效清除病原体,而持续的慢性炎症则导致组织病理损伤。核因子-κB(nuclear factor kappa-B,NF-κB)是炎症反应的关键转录调控因子,在静息状态下通过与其抑制蛋白IκB结合而被锚定于细胞质中[18]。当受到Toll样受体(Toll-like receptor,TLR)激动剂等细胞因子刺激时,IκB发生快速磷酸化降解,促使NF-κB易位进入细胞核,激活下游炎症因子基因的转录,进而引起炎症反应[19]。研究发现,在葡聚糖硫酸钠诱导的结肠炎模型中,半胱氨酸亚磺酸脱羧酶(cysteine sulfinic acid decarboxylase,CSAD)和牛磺酸转运蛋白(taurine transporter,TauT)的表达水平显著下调,且基因敲除试验证实CSADTauT缺失会加剧炎症反应;对作用机制的研究表明,牛磺酸可通过与TLR4结合,抑制NF-κB信号通路,从而降低肿瘤坏死因子-α(tumor necrosis factor-α,TNF-α)和白细胞介素-6(interleukin-6,IL-6)等促炎因子的表达[20]。此外,牛磺酸和乳酸菌联用可降低急性胰腺炎小鼠模型髓过氧化物酶(myeloperoxidase,MPO)、白细胞介素-33(interleukin-33,IL-33)、NF-κB p65和辣椒素受体(transient receptor potential vanilloid-1,TRPV-1)抗衡炎症,并明确作用机制是通过TRPV-1/IL-33/NF-κB信号转导缓解急性胰腺炎[5]。在伯氏疟原虫ANKA株感染小鼠模型中,补充牛磺酸可显著降低血清促炎细胞因子的含量,并抑制脾脏炎性小体相关基因的表达,强调了牛磺酸在青蒿素治疗患疟疾小鼠过程中的抗炎益处[21]。此外,信号转导和转录激活因子3(signal transducer and activator of transcription,STAT3)是一种调节炎症反应相关基因的转录因子,广泛参与促炎和抗炎机制[22]。在结肠炎模型中报道,牛磺酸可通过STAT3介导的促炎信号传导对结肠炎发挥保护作用[23]。在脂多糖(lipopolysaccharide,LPS)诱导的脓毒症小鼠模型中发现,牛磺酸可降低中性粒细胞和单核细胞中TNF-α和白细胞介素-1β(interleukin-1β,IL-1β)的蛋白表达水平,并通过减少中性粒细胞浸润来改善肺脏、肝脏和肾脏的损伤[24]
由此可见,牛磺酸通过抑制促炎信号传导,同时增强抗炎和可能的促溶解机制,对宿主炎症具有保护作用。

2.3 调节脂代谢能力

脂质代谢紊乱如高甘油三酯血症和高胆固醇血症是诱导心血管疾病和动脉粥样硬化的重要危险因素。牛磺酸通过多种分子机制参与脂质代谢的调控。沉寂信息调节因子1(sirtuin1,SIRT1)作为一种烟酰胺腺嘌呤二核苷(nicotinamide adenine dinucleotide,NAD+)依赖的蛋白脱酰酶,能够催化多种非组蛋白的去乙酰化修饰,在脂质代谢调控中发挥关键作用[25]。研究证实,牛磺酸干预可显著抑制高脂饮食诱导的小鼠体重增加和肝脏肥大,改善血清胆固醇和甘油三酯含量;其分子机制涉及上调肝脏组织中SIRT1活性及NAD+水平,促进SIRT1 mRNA和蛋白表达,同时抑制脂肪生成关键基因[固醇调节元件结合蛋白1c(sterol regulatory element-binding protein 1c,SREBP1c)、脂肪酸合酶(fatty acid synthase,FAS)、过氧化物酶体增殖物激活受体γ(peroxisome proliferator-activated receptor γ,PPARγ)]的表达,并激活β氧化相关基因[过氧化物酶体增殖物激活受体α(peroxisome proliferator-activated receptor α,PPARα)、肝脏X受体β(liver X receptor β,LXRβ)、过氧化物酶体增殖物激活受体γ共激活因子1α(peroxisome proliferator-activated receptor gamma coactivator 1α,PGC1α)、AMP活化蛋白激酶(AMP-activated protein kinase,AMPK)]和脂溶性调控基因[叉头框蛋白O1转录因子(forkhead box protein O1,FOXO1)],从而通过激活SIRT1/AMPK/FOXO1信号通路发挥对肥胖小鼠的降脂作用[6]。此外,小鼠长期补充牛磺酸可降低血浆中胆固醇和胆汁酸含量,上调肝脏中胆固醇7α-羟化酶(cholesterol 7-alpha hydroxylase,CYP7A1)表达水平,同时抑制ERK和成纤维细胞生长因子21(fibroblast growth factor 21,FGF21)表达水平,体外细胞试验也得出相同结果,验证了牛磺酸通过抑制FGF21/ERK通路上调Cyp7A1表达促进胆固醇代谢的机制[26]。另一研究通过细胞热位移试验、药物亲和响应靶标稳定性和双荧光素酶报告基因测定技术验证出,腺苷A2A受体(adenosine A2A receptor,A2AR)是牛磺酸的直接作用靶标,牛磺酸通过抑制A2AR-固醇调节元件结合蛋白2(sterol-regulatory element binding protein 2,SREBP-2)/环磷腺苷效应元件结合蛋白(cAMP-response element binding protein,CREB)/3-羟基-3-甲基戊二酰辅酶A还原酶(3-hydroxy-3-methylglutaryl-CoA reductase,HMGCR)轴改善胆固醇代谢失调[27]
综上可知,牛磺酸可通过SIRT1/AMPK/FOXO1、FGF21/ERK以及A2AR-SREBP-2/CREB/HMGCR等信号通路多途径、多靶点调节脂代谢紊乱,保护机体健康。

2.4 调节肠道菌群能力

肠道微生物群落作为人和动物体重要的微生物器官,其组成和功能与宿主健康密切相关。新一代测序已将其与宿主表型相关联,一系列脑/肝脏/肺脏/皮肤-肠道-微生物群轴相互作用通路正在逐渐阐明[28-30]。研究表明,牛磺酸能够显著影响肠道微生物的组成和代谢功能。在健康小鼠模型中,牛磺酸干预可特异性富集放线菌门、变形菌门、双歧杆菌属和嗜双歧杆菌属等有益菌群[31],这些菌群可能参与了牛磺酸的肠道代谢过程。值得注意的是,牛磺酸通过调节胆汁酸代谢影响肠道菌群构成,其中胆盐水解酶(bile salt hydrolase,BSH)催化的初级胆汁酸向次级胆汁酸转化是关键环节。由于乳酸菌富含BSH活性,因此在牛磺酸干预的非酒精性脂肪肝病和抗生素处理模型中表现出显著增殖优势,并促进微生物群落稳态的恢复[31-32]。研究发现,无论是天然来源还是化学合成的牛磺酸,均能提高小鼠肠道中乳杆菌属和另支菌属等有益菌的相对丰度,同时抑制幽门螺杆菌等致病菌的增殖[7]。在模拟人结肠的试验中发现,牛磺酸对门和属水平的微生物群落组成没有影响[33],这一结果与以上小鼠试验的结果形成了鲜明的对比。这种差异可能源于人类与小鼠肠道微生物组成的固有差异或试验剂量差异(小鼠研究常用165 mg/kg,而人体推荐剂量是约40 mg/kg)。值得注意的是,临床研究发现,当人类肠道微生态改善时,牛磺酸代谢通路呈现显著上调特征[34],提示牛磺酸可能在人类肠道微生态调节中发挥潜在作用。欧阳轶强等[35]研究发现,牛磺酸对乳腺癌大鼠的肠道菌群结构有调节作用,这可能与其抗肿瘤作用存在关联。
综上可知,牛磺酸可调节肠道菌群稳态,通过提高益生菌相对丰度和降低有害菌相对丰度,在维持宿主肠道健康方面发挥积极作用(表1)。
表1 牛磺酸对肠道菌群的影响

Table 1 Effects of taurine on gut microbiota

模型
Models
添加量
Additive quantity
添加途径
Additive path
影响
Effect
参考文献
References
健康小鼠
Healthy mice
200 mmol/L 饮水 放线菌门、变形菌门、双歧杆菌属、
嗜双歧杆菌属↑
[31]
健康BALB/C小鼠
Healthy BALB/C mice
165 mg/(kg·d) 灌胃 另枝菌属、紫单胞菌科、梭状
芽孢杆菌目、乳酸菌目↑,毛螺菌科、
理研菌科、螺旋杆菌科↓
[7]
抗生素致肠道菌群失调小鼠
Mice with intestinal flora imbalance caused by antibiotics
200 mmol/L 饮水 变形菌门、疣微菌门、乳杆菌属、
肠杆菌属和变形杆菌属↑
[31]
鼠疫杆菌感染小鼠
Infection of mice by Yersinia pestis
200 mmol/L 饮水 变形菌门、疣微菌门、变形杆菌属、
摩根氏菌属、乳杆菌属↑
[31]
非酒精性脂肪肝病大鼠
Rats with non-alcoholic fatty
liver disease
40 mg/(kg·d) 灌胃 双歧杆菌属、乳杆菌属↑,
大肠杆菌属↓
[32]
乳腺癌大鼠
Rats with breast cancer
6% 饮水 消化链球菌、Blautia producta、无乳链球菌、
粪肠球菌、脱硫弧菌属、Adlercreutzia↑,
Rosebura faecis、柔膜菌门、颤螺菌属↓
[35]

↑:提高 increase;↓:降低 decrease。下表同 the same as below。

3 牛磺酸在动物生产中的应用

3.1 牛磺酸对生长性能的影响

牛磺酸能有效提高动物生长以及饲料利用率等生长性能指标。在断奶仔猪的饲养试验中,饲粮中添加0.1%、0.3%和0.5%牛磺酸可剂量依赖性地提高断奶体重,其中0.3%和0.5%的添加量显著改善了仔猪的饲料转化率(FCR)[36]。在母猪上的研究表明,妊娠后期至哺乳期补充1%牛磺酸能显著提高泌乳期平均日采食量(ADFI)和仔猪断奶体重[37]。在育肥猪上的试验表明,0.2%牛磺酸添加组终末体重和平均日增重(ADG)显著提升,同时FCR呈现改善趋势[38]。在家禽生产方面,适宜剂量的牛磺酸可显著增加肉鸡[39]、肉鸭[40]以及笼养蛋雏鸭[41]的终末体重、ADG以及FCR,并能提高蛋鸡[42]的产蛋率以及平均蛋重。在反刍动物的研究中,饲粮中添加4 g/(d·头)的牛磺酸可显著提高犊牛的终末体重[43];以包被形式每天补饲25、50和75 g牛磺酸均可显著提高育肥牛的ADG[44],直接添加20和40 g牛磺酸可改善瘤胃微生物蛋白合成并提高纤维消化率,但对生长性能无显著影响[45]
综合以上研究结果可知,牛磺酸可提高畜禽的生长性能,表现为提高体重、ADG和FCR(表2)。
表2 牛磺酸对动物生长性能的影响

Table 2 Effects of taurine on growth performance of animals

动物
Animals
添加量
Additive quantity
影响
Effects
参考文献
References
猪Pigs
断奶仔猪Weaned piglets 0.5% BW↑,FCR↑ [36]
断奶仔猪Weaned piglets 1.5% ADG↓,ADFI↓ [46]
断奶仔猪Weaned piglets 0.3% BW↑,FCR↑ [47]
妊娠与哺乳期母猪Pregnant and lactating sows 1.0% BW↑,ADFI↑ [37]
育肥猪Fattening pigs 0.2% BW↑,ADG↑ [38]
家禽Poultry
肉鸡Broilers 0.5% BW↑,FCR↑ [39]
肉鸡Broilers 0.6% BW↑,FCR↑ [48]
肉鸡Broilers 0.1% ADG↑,FCR↑ [49]
蛋鸡Laying hens 0.1% 产蛋率↑,平均蛋重↑,FCR↑ [42]
肉鸭Meat ducks 0.1% BW↑,FCR↑ [40]
蛋雏鸭Laying ducklings 0.1% ADG↑,FCR↑ [41]
鹌鹑Quails 0.05% ADFI↓,FCR↑ [50]
牛Cattle
犊牛Calves 4 g/(d·头) BW↑ [43]
肉用阉牛Beef steers 75 g/(d·头) ADG↑ [44]
肉用阉牛Beef steers 40 g /(d·头)(包被形式) 对生长性能无显著影响 [45]

BW:体重 body weight;FCR:饲料转化率;feed conversion ratio;ADG:平均日增重 average daily gain;ADFI:平均日采食量:average daily feed intake。

3.2 牛磺酸对肉品质的影响

肉品质是由pH、肉色[红度(a*)、黄度(b*)、亮度(L*)值]、滴水损失、肌内脂肪(IMF)含量以及肌肉纤维类型等组成的综合性指标,是养殖业中一项重要的经济性状,直接或间接影响消费者的消费倾向。其中,肌肉纤维类型尤为重要,包括氧化型(Ⅰ型和Ⅱa型)肌纤维和糖酵解型(Ⅱb型)肌纤维,Ⅰ型肌纤维具有较低的糖原储存量和较高的pH,与滴失率呈负相关,并富含肌红蛋白,决定动物屠宰后肉的颜色。研究表明,饲粮中添加0.6%牛磺酸可通过促进Ⅱb型肌纤维向Ⅰ型肌纤维转化,显著提高pH45 min和a*值,降低滴水损失、b*和L*值,并趋于提高背最长肌中单不饱和脂肪酸和油酸(C18∶1n9c)的含量,从而改善猪肉品质[51]。此外,通过体内与体外联合研究发现,牛磺酸可通过抑制低氧诱导因子1α(hypoxia-inducible factor 1α,HIF-1α)信号通路降低猪骨骼肌糖酵解活性[52]。在肉鸡的试验中发现,牛磺酸通过介导钙调磷酸酶(calcineurin,CaN)-活化T细胞核因子(nuclear factor of activated T-cells,NFAT)信号通路诱导Ⅱb型肌纤维向Ⅰ型肌纤维转化,改善腿肌pH45 min、pH24 h、蒸煮损失以及剪切力,同时显著降低乳酸含量以及糖酵解潜力[53]。已有多项研究报道了牛磺酸在改善肉鸡[54-56]与育肥猪[38,57-58]肉品质方面的积极作用。此外,适宜剂量的牛磺酸还能提高肉鸡[59]与肉鸭[40]胸肌率和瘦肉率,降低皮下脂肪厚度,从而优化屠宰性能。
综合以上研究发现,牛磺酸可通过介导CaN-NFAT和HIF-1α信号通路促进肌纤维类型的有益转化,降低糖酵解潜力,在提高肉品质方面表现出显著效果(表3)。
表3 牛磺酸对动物肉品质的影响

Table 3 Effects of taurine on meat quality of animals

动物
Animals
添加量
Additive quantity
影响
Effects
参考文献
References


育肥猪
Fattening pigs
0.3% pH45 min↑,a*值↑,L*、b*值↓
滴水损失↓,乳酸含量↓,单不饱和脂肪酸含量↑,油酸含量↑
[53]
2 000 mg/kg pH45 min↑,a*值↑,肌红蛋白含量↑ [38]
800 mg/kg pH45 min↑,a*值↑,滴水损失↓ [57]


肉鸡
Broilers
0.5% pH45 min↑,蒸煮损失↓,剪切力↓,乳酸含量↓,
肌纤维直径↓,肌纤维密度↑
[54]
0.5% pH45 min↑,b*值↓,蒸煮损失↓,滴水损失↓ [55]
0.15% pH45 min↑,a*值↑,滴水损失↓,蛋白质含量↑,
胸肌率↑,瘦肉率↑,皮脂厚↓
[56]
肉鸭
Meat ducks
0.15% 屠宰率↑,全净膛率↑,腿肌率↑,瘦肉率↑,
腹脂率↓,系水力↑,剪切力↓
[40]

a*:红度 redness;b*:黄度 yellowness;L*:亮度 lightness。

3.3 牛磺酸对肠道健康的影响

肠道作为动物机体重要的消化吸收和免疫器官,其健康状态直接影响畜禽的生产性能。肠道屏障功能是抵御病原体和有害抗原入侵的关键防线,而肠道微生物稳态的维持对于预防组织损伤和疾病发生具有重要作用。因此,良好的肠道结构、平衡的菌群以及稳定的屏障系统是肠道生理功能的基础。在LPS以及敌草快诱导的仔猪模型试验中,牛磺酸可改善仔猪肠道的绒毛形态结构[60-63],逆转肠道紧密连接蛋白封闭蛋白-1(Claudin-1)、闭锁小带蛋白-1(ZO-1)和闭合蛋白(Occludin)mRNA表达的下调,并降低血清中二胺氧化酶(decentralized autonomous organization,DAO)活性[60-62],从而有效维护肠道形态结构与屏障功能。同时,牛磺酸能通过调节微生物群落组成(如下调拟杆菌门、螺旋体科和普雷沃氏菌科的丰度,上调厚壁菌门和乳杆菌科的丰度)来缓解LPS诱导的结肠微生态失衡[60]。在母猪[37]与育肥猪[64]试验中,牛磺酸在哺乳母猪后代与育肥猪肠道菌群稳态和肠道屏障功能方面也表现出显著的调控作用。在肉鸡试验中,饲粮中添加牛磺酸可使空肠绒毛长度以及绒毛长度与隐窝深度比值有最佳表现[65-66],并显著上调空肠ZO-1的mRNA表达水平[67]。瘤胃球菌属[68]、NK4A214_group[69]和毛螺菌属[70]可促进反刍动物体内纤维素的降解。在反刍动物上的研究显示,牛磺酸能特异性富集瘤胃中具有纤维素降解功能的微生物,如瘤胃球菌属、NK4A214_group和毛螺菌属,从而提高中性洗涤纤维的消化率[45]
综上所述,牛磺酸可改善肠道形态结构、维持肠道屏障功能以及调节肠道微生物稳态,进而保持畜禽肠道健康状态,以发挥良好的生产状态。

3.4 牛磺酸对应激的缓解作用

应激反应作为机体应对内外环境变化的非特异性生理反应,在超过适应阈值时可导致内环境紊乱并诱发多种疾病。尤其是在现代规模化、集约化畜禽养殖中,对生产性能的高要求普遍伴随多种应激,如断奶、运输、热、冷应激,严重制约畜禽生产性能的发挥。肉鸡由于羽毛丰富、缺乏汗腺和高代谢活动,特别容易受到热应激的影响[71],进而损害生长性能和肉品质[72]。有研究报道,牛磺酸可显著提高热应激肉鸡的体重[73-75]以及FCR[74,76],促进脂肪分解和蛋白质合成,并抑制胸肌蛋白质降解[76],进而减轻慢性热应激诱导的胸肌蛋白质损失[74,77-79]。在一项蛋鸡热应激的试验中,牛磺酸可提高平均产蛋率和蛋重,降低平均料蛋比,同时降低死淘率[80],还能减轻蛋鸡急性热应激诱发的输卵管损伤并增强机体免疫与抗氧化机能[81]。对热应激鹌鹑的研究表明,牛磺酸可上调回肠中营养转运蛋白的基因表达,如肽转运蛋白1(peptide transporter 1,PEPT1)、兴奋性氨基酸转运体3(excitatory amino acid transporter 3,EAAT3)、阳离子氨基酸转运蛋白2(cationic amino acid transporter 2,CAT2)、钠-葡萄糖协同转运蛋白1(sodium/glucose cotransporter 1,SGLT1)、钠-葡萄糖协同转运蛋白5(sodium/glucose cotransporter 5,SGLT5)、葡萄糖转运蛋白2(glucose transporter 2,GLUT2)和葡萄糖转运蛋白5(glucose transporter 5,GLUT5)[82]。此外,包被牛磺酸还可改善热应激种公羊精液质量,提高其繁殖性能[83-84]。慢性冷应激可诱发肉鸡氧化应激,导致心肌活性氧积累和损伤,而牛磺酸可通过上调Nrf2信号通路增强心肌抗氧化能力,对低温环境下心肌起到保护作用[85]。在断奶仔猪的研究中发现,牛磺酸可从肠道形态结构[86]、黏膜屏障和微生物菌群3个方面缓解肠道氧化损伤,进而导致腹泻程度下降[87]以及FCR升高[88-89],改善生长性能[47,90-91],缓解断奶应激的负面影响。运输应激是影响动物健康和生产性能的关键死前因素,牛磺酸可减少牦牛运输导致的体重损失,提高抗氧化能力和免疫机能,并上调瘤胃优势菌群的丰度[92]
综上所述,牛磺酸作为一种高效的畜禽饲料添加剂,在缓解应激方面展现出显著的应用潜力,其通过增强抗氧化能力、改善免疫机能、调节营养代谢和维持肠道健康等多重机制,有效提升畜禽的生长性能、繁殖能力和产品品质。

4 影响牛磺酸应用效果的因素

4.1 牛磺酸的添加剂量

饲粮中添加超过1.5%的牛磺酸会导致仔猪生长和肠道健康受损[46]。蛋氨酸和半胱氨酸的过量摄入会导致动物生长受到抑制,而牛磺酸作为蛋氨酸和半胱氨酸的代谢产物,产生类似功效并不奇怪[93]。因此,在生产应用中牛磺酸的剂量选择尤为重要。不同牛磺酸添加剂量应用效果的研究主要集中在猪和禽生产中,以生长性能相关指标为例,表2总结了不同剂量牛磺酸应用效果的相关研究。几乎所有研究表明,低剂量添加牛磺酸对动物生长性能具有显著改善效果,而过量添加的效果与不同种类动物的耐受量需深入探究。

4.2 动物生理状况

研究表明,在动物肠道菌群稳态紊乱以及机体遭受氧化应激时牛磺酸的应用效果尤为显著,主要包含动物断奶期或是应激期(温度、运输)。例如,在牛磺酸添加剂量相似时,最适温度下肉鸡FCR提高7.6%和11.1%,在热应激温度条件下提高12.3%[76]。也有研究表明,牛磺酸可显著改善断奶期仔猪生长与腹泻状况[36-37]。这主要归因于牛磺酸可提高肠道有益菌(双歧杆菌属与乳杆菌属等)丰度以及通过多途径发挥抗氧化的生物学功能。牛磺酸在动物应激状态下的调控效应更为显著,这具有重要的生产应用价值。

4.3 与其他添加剂的协同作用

研究发现,牛磺酸和二甲双胍结合使用比单独使用更能抵抗糖尿病诱导的大鼠红细胞代谢紊乱和氧化应激[94]。饲粮中添加4 mg/kg包被叶酸和40 mg/kg牛磺酸可显著提高热应激羔羊的ADG,并改善抗氧化能力和免疫水平[95]。此外,牛磺酸和乳酸菌的联用在急性胰腺炎小鼠模型中表现出显著的抗氧化与抗炎作用[5]。以上研究表明,牛磺酸与其他添加剂联合使用的互作效应在动物生产中可能具有更佳效果,但在畜牧领域相关研究报道鲜有,需进一步探究。

4.4 其他因素

其他因素包括试验动物本身的差异和牛磺酸的添加形式等。研究表明,以包被方式补充牛磺酸可提高育肥牛的ADG[44],但以直接方式补充牛磺酸对育肥牛的生长无显著影响[45]。结果产生差异可能归因于直接方式补充牛磺酸会导致大部分牛磺酸在瘤胃中被水解,剩余部分不足以发挥促生长作用。此外,动物的年龄、品种以及生长阶段不同导致的肠道菌群和吸收能力的差异都会影响牛磺酸的应用效果。

5 小结与展望

牛磺酸作为一种具有多功能的生物活性物质,在医学和其他领域的研究中已展现出其多方位的作用,包括抗氧化、抗炎、调节脂代谢和肠道菌群等。在畜牧领域,牛磺酸已被证实能够显著改善动物的生长性能、产品品质、肠道健康,并可效缓解多种应激反应,对提高动物的生产性能和健康水平具有重要应用价值。
然而,尽管牛磺酸在畜牧领域的研究已取得显著进展,但仍存在以下问题:1)牛磺酸具有多重生物学功能,其在畜禽体内的作用机制尚未完全阐明;2)牛磺酸与其他饲料添加剂的互作效应尚需研究;3)牛磺酸在反刍动物中的应用研究较少,其在反刍动物生产中的应用潜力需进一步探索。
因此,未来研究应重点关注牛磺酸在反刍动物中的应用,重点解析其对瘤胃微生物生态系统及营养物质代谢的调控规律及对肉用反刍动物脂质和蛋白质合成与分解的调节作用;应探究牛磺酸与其他益生素和抗氧化剂的联合使用效果;此外,还应整合基因组学、代谢组学和蛋白质组学等系统生物学方法,结合生物信息学分析技术,精准鉴定其分子作用靶点,深入揭示其多途径调控网络,为牛磺酸在畜牧业中的精准应用提供理论依据。
[1]
JACOBSEN J G, SMITH L H. Biochemistry and physiology of taurine and taurine derivatives[J]. Physiological Reviews, 1968, 48(2):424-511.

[2]
JONG C J, SANDAL P, SCHAFFER S W. The role of taurine in mitochondria health:more than just an antioxidant[J]. Molecules, 2021, 26(16):4913.

[3]
JIA F, YUE M, CHANDRA D, et al. Taurine is a potent activator of extrasynaptic GABA(A) receptors in the thalamus[J]. Journal of Neuroscience, 2008, 28(1):106-115.

[4]
PIAO F Y, GAO B H, YUAN X L, et al. Taurine ameliorates oxidative stress in spinal cords of diabetic rats via Keap1-Nrf2 signaling[J]. Advances in Experimental Medicine and Biology, 2022,1370:235-242.

[5]
MORES M G, FIKRY E M, EL-GENDY A O, et al. Probiotics mixture and taurine attenuate L-arginine-induced acute pancreatitis in rats:impact on transient receptor potential vanilloid-1 (TRPV-1)/IL-33/NF-κB signaling and apoptosis[J]. Tissue and Cell, 2023,85:102234.

[6]
KARIKKAKKAVIL PRAKASHAN A D, MUTHUKUMAR S P, MARTIN A. Taurine activates SIRT1/AMPK/FOXO1 signaling pathways to favorably regulate lipid metabolism in C57BL6 obese mice[J]. Molecular Nutrition & Food Research, 2024, 68(8):e2200660.

[7]
YU H N, GUO Z Z, SHEN S R, et al. Effects of taurine on gut microbiota and metabolism in mice[J]. Amino Acids, 2016, 48(7):1601-1617.

[8]
MOTAWI T K, ABD ELGAWAD H M, SHAHIN N N. Modulation of indomethacin-induced gastric injury by spermine and taurine in rats[J]. Journal of Biochemical and Molecular Toxicology, 2007, 21(5):280-288.

[9]
RAMALINGAM M, KIM S J. Reactive oxygen/nitrogen species and their functional correlations in neurodegenerative diseases[J]. Journal of Neural Transmission, 2012, 119(8):891-910.

[10]
QU J, LIU K, LIU S P, et al. Taurine alleviates ochratoxin A-induced pyroptosis in PK-15 cells by inhibiting oxidative stress[J]. Journal of Biochemical and Molecular Toxicology, 2023, 37(2):e23249.

[11]
BUENDIA I, MICHALSKA P, NAVARRO E, et al. Nrf2-ARE pathway:an emerging target against oxidative stress and neuroinflammation in neurodegenerative diseases[J]. Pharmacology & Therapeutics, 2016,157:84-104.

[12]
CHEN X P, LIU J, CHEN S Y. Over-expression of Nrf2 diminishes ethanol-induced oxidative stress and apoptosis in neural crest cells by inducing an antioxidant response[J]. Reproductive Toxicology, 2013,42:102-109.

[13]
HONG C L, CAO J M, WU C F, et al. The Chinese herbal formula free and easy wanderer ameliorates oxidative stress through KEAP1-NRF2/HO-1 pathway[J]. Scientific Reports, 2017, 7(1):11551.

[14]
XU M M, CHE L, GAO K G, et al. Taurine alleviates oxidative stress in porcine mammary epithelial cells by stimulating the Nrf2-MAPK signaling pathway[J]. Food Science & Nutrition, 2023, 11(4):1736-1746.

[15]
WU G F, SAN J S, PANG H P, et al. Taurine attenuates AFB1-induced liver injury by alleviating oxidative stress and regulating mitochondria-mediated apoptosis[J]. Toxicon, 2022,215:17-27.

[16]
CHEN B T, ABAYDULA Y, LI D L, et al. Taurine ameliorates oxidative stress by regulating PI3K/Akt/GLUT4 pathway in HepG2 cells and diabetic rats[J]. Journal of Functional Foods, 2021,85:104629.

[17]
LOU J, HAN D H, YU H H, et al. Cytoprotective effect of taurine against hydrogen peroxide-induced oxidative stress in UMR-106 cells through the Wnt/β-catenin signaling pathway[J]. Biomolecules & Therapeutics, 2018, 26(6):584-590.

[18]
LUEDDE T, SCHWABE R F. NF-κB in the liver-linking injury,fibrosis and hepatocellular carcinoma[J]. Nature Reviews Gastroenterology & Hepatology, 2011, 8(2):108-118.

[19]
HE A Q, JI R, SHAO J, et al. TLR4-MyD88-TRAF6-TAK1 complex-mediated NF-κB activation contribute to the anti-inflammatory effect of V8 in LPS-Induced human cervical cancer SiHa cells[J]. Inflammation, 2016, 39(1):172-181.

[20]
ZHENG J M, ZHANG J L, ZHOU Y W, et al. Taurine alleviates experimental colitis by enhancing intestinal barrier function and inhibiting inflammatory response through TLR4/NF-κB signaling[J]. Journal of Agricultural and Food Chemistry, 2024, 72(21):12119-12129.

[21]
LI X, JIANG N, LI Q L, et al. Taurine potentiates artemisinin efficacy against malaria by modulating the immune response in Plasmodium berghei-infected mice[J]. Parasites & Vectors, 2024, 17(1):493.

[22]
O'SHEA J J, MURRAY P J. Cytokine signaling modules in inflammatory responses[J]. Immunity, 2008, 28(4):477-487.

[23]
KIM S H, YUM H W, KIM S H, et al. Protective effects of taurine chloramine on experimentally induced colitis:NFκB,STAT3,and Nrf2 as potential targets[J]. Antioxidants, 2021, 10(3):479.

[24]
MA Y, ZHANG Y, LI R, et al. Mechanism of taurine reducing inflammation and organ injury in sepsis mice[J]. Cellular Immunology, 2022,375:104503.

[25]
LOMB D J, LAURENT G, HAIGIS M C. Sirtuins regulate key aspects of lipid metabolism[J]. Biochimica et Biophysica Acta:Proteins and Proteomics, 2010, 1804(8):1652-1657.

[26]
TAGAWA R, KOBAYASHI M, SAKURAI M, et al. Long-term dietary taurine lowers plasma levels of cholesterol and bile acids[J]. International Journal of Molecular Sciences, 2022, 23(3):1793.

[27]
CHEN B B, BAO R X, PAN J J, et al. Taurine alleviates dysfunction of cholesterol metabolism under hyperuricemia by inhibiting A2AR-SREBP-2/CREB/HMGCR axis[J]. Journal of Lipid Research, 2025, 66(2):100746.

[28]
ANAND S, MANDE S S. Diet,microbiota and gut-lung connection[J]. Frontiers in Microbiology, 2018,9:2147.

[29]
DANG A T, MARSLAND B J. Microbes,metabolites,and the gut-lung axis[J]. Mucosal Immunology, 2019, 12(4):843-850.

[30]
MAHMUD M R, AKTER S, TAMANNA S K, et al. Impact of gut microbiome on skin health:gut-skin axis observed through the lenses of therapeutics and skin diseases[J]. Gut Microbes, 2022, 14(1):2096995.

[31]
QIAN W K, LI M Y, YU L L, et al. Effects of taurine on gut microbiota homeostasis:an evaluation based on two models of gut dysbiosis[J]. Biomedicines, 2023, 11(4):1048.

[32]
ZHU F L, HUANG T, LV Z L, et al. Taurine regulates the expression of interleukin-17/10 and intestinal flora and protects the liver and intestinal mucosa in a nonalcoholic fatty liver disease rat model[J]. Diabetes,Metabolic Syndrome and Obesity, 2024,17:675-689.

[33]
SASAKI K, SASAKI D, OKAI N, et al. Taurine does not affect the composition,diversity,or metabolism of human colonic microbiota simulated in a single-batch fermentation system[J]. PLoS One, 2017, 12(7):e0180991.

[34]
HUANG Y H, CHANG L C, CHANG Y C, et al. Compositional alteration of gut microbiota in psoriasis treated with IL-23 and IL-17 inhibitors[J]. International Journal of Molecular Sciences, 2023, 24(5):4568.

[35]
欧阳轶强, 宋玉美, 梁柏莹, 等. 牛磺酸对乳腺癌大鼠肠道菌群的影响[J]. 广西医科大学学报, 2017, 34(4):491-495.

OUYANG Y Q, SONG Y M, LIANG B Y, et al. The influence of taurine on gut microbes in breast cancer model rats[J]. Journal of Guangxi Medical University, 2017, 34(4):491-495. (in Chinese)

[36]
CHEN J J, ZHANG X F, ZHANG Y H, et al. Taurine enhances growth performance by improving intestinal integrity and antioxidant capacity of weaned piglets[J]. Journal of Animal Science, 2024,102:skae311.

[37]
XU M M, CHE L, GAO K G, et al. Effects of dietary taurine supplementation to gilts during late gestation and lactation on offspring growth and oxidative stress[J]. Animals, 2019, 9(5):220.

[38]
李永明, 门小明, 陶新, 等. 牛磺酸对育肥猪生长性能、肉品质、抗氧化功能及肌肉能量代谢的影响[J]. 动物营养学报, 2023, 35(2):803-812.

LI Y M, MEN X M, TAO X, et al. Effects of taurine on growth performance,meat quality,antioxidant function and muscle energy metabolism of finishing pigs[J]. Chinese Journal of Animal Nutrition, 2023, 35(2):803-812. (in Chinese)

[39]
HAN H L, ZHANG J F, YAN E F, et al. Effects of taurine on growth performance,antioxidant capacity,and lipid metabolism in broiler chickens[J]. Poultry Science, 2020, 99(11):5707-5717.

[40]
臧素敏, 李同洲, 郭鹏飞. 添加牛磺酸对樱桃谷肉鸭生产性能和肌肉品质影响的研究[J]. 中国家禽, 2007, 29(24):12-15.

ZANG S M, LI T Z, GUO P F. Effect of dietary taurine on the production performance and meat quality in cherry valley meat duck[J]. China Poultry, 2007, 29(24):12-15. (in Chinese)

[41]
杨小然, 王安, 郭志杰. 牛磺酸对笼养蛋雏鸭生长性能、抗氧化功能及免疫器官发育的影响[J]. 动物营养学报, 2011, 23(5):807-812.

YANG X R, WANG A, GUO Z J. Effects of taurine on growth performance,antioxidant function and immune organ development of caged egg-type ducklings[J]. Chinese Journal of Animal Nutrition, 2011, 23(5):807-812. (in Chinese)

[42]
姚海飞, 易军, 包德威. 牛磺酸对蛋鸡生产性能及免疫机能的影响[J]. 家禽科学, 2023, 45(11):44-47.

YAO H F, YI J, BAO D W. Effects of taurine on performance and immune function of laying hens[J]. China Poultry Science, 2023, 45(11):44-47. (in Chinese)

[43]
田雨晴, 张一平, 吴春会, 等. 低聚木糖和牛磺酸对犊牛生长性能、腹泻率和营养物质表观消化率的影响[J]. 动物营养学报, 2024, 36(1):374-386.

TIAN Y Q, ZHANG Y P, WU C H, et al. Effects of xylo-oligosaccharides and taurine on growth performance,diarrhea rate and nutrient apparent digestibility of calves[J]. Chinese Journal of Animal Nutrition, 2024, 36(1):374-386. (in Chinese)

[44]
ZHANG S, HU J M, LIU Y F, et al. Taurine drives body protein renewal and accretion in beef steers[J]. Animal Nutrition, 2024,19:1-12.

[45]
LIU Y F, HU J M, LI M M, et al. Effects of taurine on rumen fermentation,nutrient digestion,rumen bacterial community and metabolomics and nitrogen metabolism in beef steers[J]. Journal of the Science of Food and Agriculture, 2023, 103(7):3414-3426.

[46]
LIU Y, MAO X B, YU B, et al. Excessive dietary taurine supplementation reduces growth performance,liver and intestinal health of weaned pigs[J]. Livestock Science, 2014,168:109-119.

[47]
ZHOU M, WU Z C, DENG D H, et al. Effects of taurine on the growth performance,diarrhea,oxidative stress and intestinal barrier function of weanling piglets[J]. Frontiers in Veterinary Science, 2024,11:1436282.

[48]
LV Q F, SUN L, CUI Y Q, et al. Effects of replacement of methionine in diets with taurine on growth performance and blood index in broilers[J]. Advances in Experimental Medicine and Biology, 2017,975:989-1000.

[49]
曾得寿, 高振华, 赵京辉, 等. 牛磺酸对肉仔鸡生产性能、免疫器官发育及抗氧化能力的影响[J]. 中国兽医学报, 2009, 29(6):774-778.

ZENG D S, GAO Z H, ZHAO J H, et al. Effects of taurine on growth performance,immune organ development and antioxidative ability of broilers[J]. Chinese Journal of Veterinary Science, 2009, 29(6):774-778. (in Chinese)

[50]
WANG F R, DONG X F, TONG J M, et al. Effects of dietary taurine supplementation on growth performance and immune status in growing Japanese quail (Coturnix coturnix japonica)[J]. Poultry Science, 2009, 88(7):1394-1398.

[51]
AN W T, HUANG Z Q, MAO Z Y, et al. Dietary taurine supplementation improves the meat quality,muscle fiber type,and mitochondrial function of finishing pigs[J]. Journal of Agricultural and Food Chemistry, 2023, 71(41):15331-15340.

[52]
CHEN X L, AN W T, HUANG Z Q, et al. Taurine reduces glycolysis of pig skeletal muscle by inhibiting HIF-1α signaling[J]. Journal of Cellular Physiology, 2025, 240(1):e31461.

[53]
徐苏微, 邢通, 李蛟龙, 等. 牛磺酸对肉鸡肉品质、糖酵解潜力及肌纤维特性的影响[J]. 南京农业大学学报, 2020, 43(5):935-941.

XU S W, XING T, LI J L, et al. Effects of dietary taurine supplementation on meat quality,glycolyticpotential and muscle fiber characteristics in broiler chickens[J]. Journal of Nanjing Agricultural University, 2020, 43(5):935-941. (in Chinese)

[54]
XU S W, LU Z, MA B B, et al. Dietary taurine supplementation enhances antioxidative capacity and improves breast meat quality of broiler chickens[J]. British Poultry Science, 2020, 61(2):140-145.

[55]
韩红丽, 张婧菲, 沈明明, 等. 牛磺酸对肉鸡生长性能、肉品质及肌肉抗氧化功能的影响[J]. 食品科学, 2020, 41(17):17-22.

HAN H L, ZHANG J F, SHEN M M, et al. Effect of taurine on growth performance,meat quality and muscle antioxidant function in broilers[J]. Food Science, 2020, 41(17):17-22. (in Chinese)

[56]
曾得寿, 高振华, 黄晓亮. 牛磺酸对肉仔鸡屠宰性能和肌肉品质的影响[J]. 中国饲料, 2011(17):21-23,28.

ZENG D S, GAO Z H, HUANG X L. Effects of taurine on slaughter performance and meat quality of broilers[J]. China Feed, 2011(17):21-23,28. (in Chinese)

[57]
孙启峰. 牛磺酸对育肥猪肉品质的影响[J]. 特种经济动植物, 2024, 27(1):23-25.

SUN Q F. Effects of taurine on meat quality of finishing pigs[J]. Special Economic Animal and Plant, 2024, 27(1):23-25. (in Chinese)

[58]
布占营. 牛磺酸对育肥猪肉品质的影响[J]. 中国动物保健, 2024, 26(10):60-61.

BU Z Y. Effects of taurine on meat quality of finishing pigs[J]. China Animal Health, 2024, 26(10):60-61. (in Chinese)

[59]
李万军. 牛磺酸对肉鸡饲粮养分利用率、免疫器官发育及屠宰性能的影响研究[J]. 中国农学通报, 2012, 28(23):6-10.

LI W J. Effect of taurine on nutrient utilization of ration,development of immune organs and slaughter performance in broiler chicken[J]. Chinese Agricultural Science Bulletin, 2012, 28(23):6-10. (in Chinese)

[60]
ZHAO D D, GAI Y D, LI C, et al. Dietary taurine effect on intestinal barrier function,colonic microbiota and metabolites in weanling piglets induced by LPS[J]. Frontiers in Microbiology, 2023,14:1259133.

[61]
MA Y D, LV Q F, ZHAO D D, et al. Intervention effect of taurine on LPS-induced intestinal mechanical barrier injury in piglets[J]. Advances in Experimental Medicine and Biology, 2022,1370:73-80.

[62]
WEN C Y, GUO Q P, WANG W L, et al. Taurine alleviates intestinal injury by mediating tight junction barriers in diquat-challenged piglet models[J]. Frontiers in Physiology, 2020,11:449.

[63]
TANG Z R, LIU J Y, SUN Z H, et al. Protective effects of taurine on growth performance and intestinal epithelial barrier function in weaned piglets challenged without or with lipopolysaccharide[J]. Animal Production Science, 2018, 58(11):2011-2020.

[64]
易山婷. 牛磺酸对育肥猪生产性能和肠道屏障功能的影响[D]. 硕士学位论文. 雅安: 四川农业大学, 2024.

YI S T. Effects of taurine on production performance and intestinal barrier function in finishing pigs[D]. Master's Thesis. Ya'an: Sichuan Agricultural University, 2024. (in Chinese)

[65]
SANDOGHDAR T, IRANI M, GHARAHVEYSI S. Taurine amino acid supplementation impacts performance,blood hematology,oxidative stress,and jejunum morphology in broiler chickens[J]. Tropical Animal Health and Production, 2024, 56(3):123.

[66]
FERNANDES J I M, RORIG A, GOTTARDO E T, et al. Post-hatch diets supplemented with sources of fat and added taurine and glycine on the intestinal morphology and performance of broilers at 1 to 21 days[J]. Arquivo Brasileiro de Medicina Veterinaria e Zootecnia, 2017, 69(1):198-204.

[67]
张国欣, 杨其峰, 刘小艳, 等. 黄芪多糖和牛磺酸饮水剂对肉鸡生长性能、抗氧化功能、免疫指标和肠道屏障功能的影响[J]. 中国家禽, 2024, 46(1):49-55.

ZHANG G X, YANG Q F, LIU X Y, et al. Effects of Astragalus polysaccharide and taurine drinking agents on growth performance,antioxidant function,immune function and intestinal barrier function in broiler chickens[J]. China Poultry, 2024, 46(1):49-55. (in Chinese)

[68]
LA REAU A J, MEIER-KOLTHOFF J P, SUEN G. Sequence-based analysis of the genus Ruminococcus resolves its phylogeny and reveals strong host association[J]. Microbial Genomics, 2016, 2(12):e000099.

[69]
YU S B, ZHANG G Y, LIU Z B, et al. Repeated inoculation with fresh rumen fluid before or during weaning modulates the microbiota composition and co-occurrence of the rumen and colon of lambs[J]. BMC Microbiology, 2020, 20(1):29.

[70]
RUSSELL J B, RYCHLIK J L. Factors that alter rumen microbial ecology[J]. Science, 2001, 292(5519):1119-1122.

[71]
VARASTEH S, BRABER S, AKBARI P, et al. Differences in susceptibility to heat stress along the chicken intestine and the protective effects of galacto-oligosaccharides[J]. PLoS One, 2015, 10(9):e0138975.

[72]
LU Z, HE X F, MA B B, et al. Chronic heat stress impairs the quality of breast-muscle meat in broilers by affecting redox status and energy-substance metabolism[J]. Journal of Agricultural and Food Chemistry, 2017, 65(51):11251-11258.

[73]
SHIM K S, HWANG K T, SON M W, et al. Lipid metabolism and peroxidation in broiler chicks under chronic heat stress[J]. Asian-Australasian Journal of Animal Sciences, 2006, 19(8):1206-1211.

[74]
HAFEEZ A, AKRAM W, SULTAN A, et al. Effect of dietary inclusion of taurine on performance,carcass characteristics and muscle micro-measurements in broilers under cyclic heat stress[J]. Italian Journal of Animal Science, 2021, 20(1):872-877.

[75]
李晓利. 牛磺酸对持续热应激肉鸡生长性能和免疫功能的影响[J]. 国外畜牧学(猪与禽), 2023, 43(2):64-66.

LI X L. Effects of taurine on growth performance and immune function of broilers under chronic heat stress[J]. Animal Science Abroad (Pigs and Poultry), 2023, 43(2):64-66. (in Chinese)

[76]
LU Z, HE X F, MA B B, et al. The alleviative effects and related mechanisms of taurine supplementation on growth performance and carcass characteristics in broilers exposed to chronic heat stress[J]. Poultry Science, 2019, 98(2):878-886.

[77]
LU Z, HE X F, MA B B, et al. Dietary taurine supplementation improves breast meat quality in chronic heat-stressed broilers via activating the Nrf2 pathway and protecting mitochondria from oxidative attack[J]. Journal of the Science of Food and Agriculture, 2019, 99(3):1066-1072.

[78]
MA B B, ZHANG L, LI J L, et al. Dietary taurine supplementation ameliorates muscle loss in chronic heat stressed broilers via suppressing the perk signaling and reversing endoplasmic reticulum-stress-induced apoptosis[J]. Journal of the Science of Food and Agriculture, 2021, 101(5):2125-2134.

[79]
LU Z, HE X F, MA B B, et al. Dietary taurine supplementation decreases fat synthesis by suppressing the liver X receptor α pathway and alleviates lipid accumulation in the liver of chronic heat-stressed broilers[J]. Journal of the Science of Food and Agriculture, 2019, 99(13):5631-5637.

[80]
任剑, 赵恒寿. 复方牛磺酸可溶性粉缓解蛋鸡热应激的效果[J]. 家禽科学, 2007(6):33-34.

REN J, ZHAO H S. Effect of compound taurine soluble powder on alleviating heat stress in laying hens[J]. Poultry Science, 2007(6):33-34. (in Chinese)

[81]
卢宇, 贾雪波, 张金秋, 等. 牛磺酸对急性热应激蛋鸡输卵管损伤的保护作用[J]. 江苏农业学报, 2011, 27(4):807-812.

LU Y, JIA X B, ZHANG J Q, et al. Protection of layer oviduct under acute heat stress by taurine[J]. Jiangsu Journal of Agricultural Sciences, 2011, 27(4):807-812. (in Chinese)

[82]
ORHAN C, KUCUK O, SAHIN N, et al. Effects of taurine supplementation on productive performance,nutrient digestibility and gene expression of nutrient transporters in quails reared under heat stress[J]. Journal of Thermal Biology, 2020,92:102668.

[83]
班斌. 叶酸和牛磺酸对热应激种公羊精液质量、血清和精浆抗氧化能力、生殖激素的影响[D]. 硕士学位论文. 晋中: 山西农业大学, 2022.

BAN B. Effects of folic acid and taurine on semen quality,serum and seminal plasma antioxidant capacity,and reproductive hormones of heat-stressed breeding rams[D]. Master's Thesis. Jinzhong: Shanxi Agricultural University, 2022. (in Chinese)

[84]
雷铭凯. 叶酸和牛磺酸对热应激绵羊睾丸生理功能和精液品质的影响[D]. 硕士学位论文. 晋中: 山西农业大学, 2023.

LEI M K. Effects of folic acid and taurine on testicular physiological function and semen quality of rams under heat stress[D]. Master's Thesis. Jinzhong: Shanxi Agricultural University, 2023. (in Chinese)

[85]
李丽杰. 牛磺酸对低温环境下肉鸡心肌抗氧化作用影响的研究[D]. 硕士学位论文. 沈阳: 沈阳农业大学, 2020.

LI L J. Study on the effect of taurine on the antioxidative effect of broiler myocardium under low temperature[D]. Master's Thesis. Shenyang: Shenyang Agricultural University, 2020. (in Chinese)

[86]
张建斌, 车向荣, 陈娟娟. 谷氨酰胺和牛磺酸对仔猪肠黏膜形态的影响[J]. 饲料研究, 2011(8):50-52.

ZHANG J B, CHE X R, CHEN J J. Effects of glutamine and taurine on intestinal mucosal morphology of piglets[J]. Feed Research, 2011(8):50-52. (in Chinese)

[87]
尚芳. 牛磺酸对断奶仔猪腹泻、消化的影响[J]. 养殖技术顾问, 2013(11):58.

SHANG F. Effects of taurine on diarrhea and digestion in weaned piglets[J]. Technical Advisor for Animal Husbandry, 2013(11):58. (in Chinese)

[88]
王林岗. 日粮添加牛磺酸对断奶仔猪肠道健康和生长性能的影响[D]. 硕士学位论文. 重庆: 西南大学, 2024.

WANG L G. Effects of dietary taurine supplementation on intestinal health and growth performance in weaned piglets[D]. Master's Thesis. Chongqing: Southwest University, 2024. (in Chinese)

[89]
张小龙. 牛磺酸对早期断奶仔猪生长性能和肠道发育的影响及机制[D]. 硕士学位论文. 重庆: 西南大学, 2015.

ZHANG X L. Study on the roles and mechanisms of taurine on growth performance and intestinal development of post-weaning piglets[D]. Master's Thesis. Chongqing: Southwest University, 2015. (in Chinese)

[90]
WANG L G, JIANG L W, CHU Y Y, et al. Dietary taurine improves growth performance and intestine health via the GSH/GSSG antioxidant system and Nrf2/ARE signaling pathway in weaned piglets[J]. Antioxidants, 2023, 12(10):1852.

[91]
李雪, 张红梅, 翟伟, 等. 日粮中添加牛磺酸对断奶仔猪生长性能、血清生化指标和免疫功能的影响[J]. 今日畜牧兽医, 2023, 39(5):11-13.

LI X, ZHANG H M, ZHAI W, et al. Effects of dietary taurine supplementation on growth performance,serum biochemical parameters and immune function in weaned piglets[J]. Today Animal Husbandry and Veterinary Medicine, 2023, 39(5):11-13. (in Chinese)

[92]
赵凯强. 日粮过瘤胃葡萄糖和牛磺酸水平对牦牛运输应激及生长性能的影响[D]. 硕士学位论文. 雅安: 四川农业大学, 2024.

ZHAO K Q. The effects of rumen-protected glucose and taurine levels in the diet on transport stress and growth performance of yaks[D]. Master's Thesis. Ya'an: Sichuan Agricultural University, 2024. (in Chinese)

[93]
BAKER D H. Comparative species utilization and toxicity of sulfur amino acids[J]. Journal of Nutrition, 2006, 136(Suppl.6):1670S-1675S.

[94]
BUDHRAM R, PANDYA K G, LAU-CAM C A. Evaluation of the actions of metformin and taurine,singly and in combination,on metabolic and oxidative alterations caused by diabetes in rat erythrocytes and plasma[J]. Advances in Experimental Medicine and Biology, 2015,803:251-270.

[95]
LI B B, WU K, DUAN G Q, et al. Folic acid and taurine alleviate the impairment of redox status,immunity,rumen microbial composition and fermentation of lambs under heat stress[J]. Animals, 2024, 14(7):998.

文章导航

/