综述

中性粒细胞胞外陷阱在畜禽健康中的作用及其营养调控研究进展

  • 周佳 ,
  • 张丽 ,
  • 曾钰 ,
  • 董贤文 , *
展开
  • 重庆市畜牧科学院, 重庆 402460
* 董贤文,研究员,E-mail:

周 佳(1992—),男,湖北黄冈人,助理研究员,博士,主要从事反刍动物营养研究。E-mail:

收稿日期: 2025-05-30

  网络出版日期: 2025-12-13

基金资助

重庆市财政资金项目(25504C)

重庆市财政资金项目(24516C)

重庆市技术创新与应用发展专项面上项目(CSTB2024TIAD-LDX0006)

重庆市技术创新与应用发展专项面上项目(CSTB2025TIAD-GPX0002)

Research Progress on Role of Neutrophil Extracellular Traps in Livestock and Poultry Health and Its Nutritional Regulation

  • ZHOU Jia ,
  • ZHANG Li ,
  • ZENG Yu ,
  • DONG Xianwen , *
Expand
  • Chongqing Academy of Animal Sciences, Chongqing 402460, China
* professor, E-mail:

Received date: 2025-05-30

  Online published: 2025-12-13

摘要

中性粒细胞胞外陷阱(NETs)作为中性粒细胞释放的DNA纤维网状结构,在病原防御中发挥双重角色:适度形成有助于捕获和清除病原体,而过度释放则通过释放蛋白酶、活性氧等效应分子加剧组织损伤和炎症反应。在畜禽生产中,多种因素如病原感染、代谢性疾病及生殖活动(如受孕)等均可诱发NETs的形成。近年来,利用营养策略调控NETs的形成逐渐受到关注。本文综述了NETs在畜禽健康中的生物学功能与作用机制,并探讨了营养干预策略调控NETs形成的应用前景,以期为防治NETs相关疾病和推动健康养殖实践提供理论依据。

本文引用格式

周佳 , 张丽 , 曾钰 , 董贤文 . 中性粒细胞胞外陷阱在畜禽健康中的作用及其营养调控研究进展[J]. 动物营养学报, 2025 , 37(12) : 8055 -8066 . DOI: 10.12418/CJAN2025.655

Abstract

Neutrophil extracellular traps (NETs), which are DNA-based fibrous networks released by neutrophils, play a dual role in pathogen defense: moderate formation helps capture and eliminate pathogens, whereas excessive release exacerbates tissue damage and inflammatory responses by releasing effector molecules such as proteases and reactive oxygen species. In livestock and poultry production, various factors including pathogen infection, metabolic diseases, and reproductive activities (such as conception) can induce the formation of NETs. In recent years, there has been growing interest in utilizing nutritional strategies to regulate NETs formation. This review summarizes the biological functions and mechanisms of NETs in livestock and poultry health, and discusses the potential application of nutritional interventions in modulating NETs formation, aiming to provide a theoretical basis for preventing and treating NETs-related diseases and promoting healthy farming practices.

在机体的免疫防御体系中,中性粒细胞作为先天性免疫的关键效应细胞,其经典抗菌功能主要包括吞噬作用和脱颗粒作用。2004年,Brinkmann等[1]在《Science》上首次报道了中性粒细胞的一种新型免疫防御机制:在病原体刺激下,中性粒细胞可通过一种独特的程序性死亡方式,释放由解聚染色质DNA、组蛋白以及多种抗菌蛋白[如髓过氧化物酶(myeloperoxidase,MPO)、中性粒细胞弹性蛋白酶(neutrophil elastase,NE)等]构成的纤维网状结构。该结构被命名为“中性粒细胞胞外诱捕网”(neutrophil extracellular traps,NETs),中文亦称“中性粒细胞胞外陷阱”。这一过程伴随特征性的细胞形态变化,既不同于细胞凋亡(表现为细胞皱缩和凋亡小体形成),也区别于坏死(以细胞膜破裂和内容物释放为特征)[2],后被学术界正式定义为一种炎性细胞死亡方式,即NETosis[3]。随着研究的不断深入,NETs的生物学功能已从最初的抗感染作用拓展至包括无菌性炎症、自身免疫性疾病、肿瘤转移及组织损伤等多种病理过程[4-5]。尽管目前关于NETs的形成机制及其病理效应的认识主要基于人类和模式动物的研究,但该现象在鸡[6]、猪[7]、羊[8]、牛[9]、骆驼[10]等畜禽动物中也已得到明确表型特征。畜禽动物在养殖过程中常面临病原感染、环境应激和营养代谢等多重免疫挑战。研究表明,NETs通过其既能捕获病原体又可介导炎症损伤的双重作用机制,在畜禽动物特异性免疫防御及相关病理性损伤中扮演关键角色[11-12]。近年研究发现,营养干预在体外可有效调控NETs的形成[13-14],为畜禽动物健康养殖提供了新的策略思路。本文就NETs在畜禽动物健康中的作用及营养调控的研究进展进行了综述,旨在为改善畜禽动物健康和生产性能提供参考。

1 NETs的形成机制及生物学特性

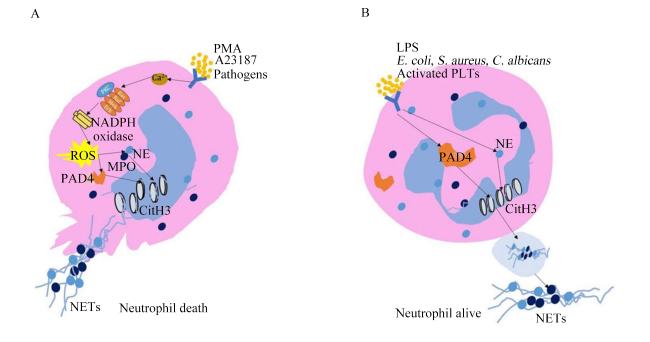
中性粒细胞在从病原体激活、组织迁移到免疫调节、微生物杀灭及NETs形成的整个免疫应答过程中表现出高度进化保守性[15]。中性粒细胞通过其表面模式识别受体(pattern recognition receptor,PRR)系统精确识别病原体相关分子模式(pathogen-associated molecular patterns,PAMPs)和损伤相关分子模式(damage-associated molecular patterns,DAMPs)。目前已明确的NETs形成机制可根据其对还原型烟酰胺腺嘌呤二核苷酸磷酸氧化酶(nicotinamide adenine dinucleotide phosphate oxidase, NOX)的依赖性分为NOX依赖性途径和非依赖性途径[16-17](图1)。在NOX依赖性途径中,病原体或炎性刺激可激活NOX,产生活性氧(reactive oxygen species,ROS),进而促使MPO和NE从颗粒中释放并进入细胞核,并通过肽酰精氨酸脱亚氨酶4(peptidylarginine deiminase 4,PAD4)介导的组蛋白瓜氨酸化导致染色质解聚和核膜破裂,最终释放NETs[18-19]。该过程中细胞内钙离子(Ca2+)浓度显著升高[20]。研究表明,NOX2介导产生的超氧阴离子及其衍生物过氧化氢在NETs形成的信号级联反应中发挥核心调控作用[21-22]。在ROS等效应分子的作用下,PAD4特异性催化组蛋白H3和H4的精氨酸残基发生瓜氨酸化修饰[23]。而非依赖性途径则通过Toll样受体(Toll-like receptors, TLR)感知信号,快速释放由氧化线粒体DNA构成的NETs[24-25]。NETs的释放方式根据刺激类型和强度可分为2种形式[26-27]:自杀型/溶解性NETosis以细胞膜完整性完全丧失、核膜破裂和细胞内容物彻底释放为特征,中性粒细胞死亡(图1-A);而活力型/非溶解性NETosis则能维持细胞核和细胞膜的完整性,通过囊泡运输途径选择性释放NETs成分(图1-B)。在NETs体外诱导模型中,佛波酯(phorbol 12-myristate 13-acetate,PMA)通过激活NOX2依赖性途径[28]、金黄色葡萄球菌通过PAMPs[8]以及脂多糖(lipopolysaccharide,LPS)通过TLR4信号通路[29],均可在适当条件下于2~4 h内高效诱导中性粒细胞形成NETs,为研究NETosis的分子机制和相关疾病治疗靶点提供了重要的体外模型。电子显微镜观察显示,成熟的NETs由直径15~17 nm的DNA纤维构成三维网状骨架,其上规律分布着直径约25 nm的球形蛋白聚集体,这种独特的网状结构可扩展至原细胞体积的15倍,在感染部位形成有效的物理屏障[30-31]。这些形成机制与结构特性是理解NETs在畜禽免疫防御与炎症损伤中的基础,也为通过营养策略靶向调控NETs以改善健康提供了关键理论依据。
图1 中性粒细胞胞外陷阱形成机制的示意图

A: 自杀型/溶解性NETosis suicidal/lytic NETosis; B:活力型/非溶解性NETosis vital/non-Lytic NETosis。Pathogens: 病原体;PMA: 佛波酯 phorbol 12-myristate 13-acetate; NADPH oxidase: 还原型烟酰胺腺嘌呤二核苷酸磷酸氧化酶 nicotinamide adenine dinucleotide phosphate oxidase; ROS: 活性氧 reactive oxygen species; NE: 中性粒细胞弹性蛋白酶 neutrophil elastase; MPO: 髓过氧化物酶 myeloperoxidase; PAD4: 肽酰精氨酸脱亚氨酶4 peptidylarginine deiminase 4; CitH3: 瓜氨酸组蛋白H3 citrullinated Histone H3; NETs: 中性粒细胞胞外陷阱 neutrophil extracellular traps; Neutrophil death: 中性粒细胞死亡; LPS: 脂多糖 lipopolysaccharide; E. coli: 大肠杆菌 Escherichia coli; S. aureus: 金黄色葡萄球菌 Staphylococcus aureus; C. albicans: 白色念球菌 Candida albicans; Activated PLTs: 活化的血小板 activated platelets; Neutrophil alive: 中性粒细胞存活。

Fig.1 Schematic illustration of formation mechanism of neutrophil extracellular traps[32]

2 畜禽生产中NETs形成的诱导因素

2.1 病原体感染

病原体感染是诱导畜禽动物体内NETs形成的主要因素之一,这一过程表现出明显的病原特异性。多种常见畜禽病原体(包括细菌、真菌、支原体、寄生虫和病毒)均可通过其特有的分子模式激活中性粒细胞,诱导NETs的生成[33]。细菌主要借助其表面结构成分激活中性粒细胞释放NETs。这些成分包括肽聚糖[1]、LPS[34]、脂磷壁酸[35]及鞭毛[36]等。真菌则通过细胞壁组分(如β-葡聚糖[37]、甘露聚糖[38])、信号分子(如法尼醇[39])及形态特征(如分生孢子和菌丝[40-41])诱导NETs形成。此外,寄生虫的细胞外囊泡[42]以及病毒与模式识别受体的相互作用[43-44]也被证实参与NETs的诱导过程。病原体的识别主要依赖于中性粒细胞表面的模式识别受体系统,包括TLR4[45-46]、核苷酸结合寡聚化结构域样受体(nucleotide-binding and oligomerization domain-like receptors,NLRs)[47]、C型凝集素受体(C-type lectin receptors,CLRs)[48]、补体受体(complement receptors,CRs)[49]以及蛋白酶激活受体2(protease-activated receptor 2,PAR2)[50]。不同病原体通过激活不同受体触发下游信号级联反应,其机制存在显著差异。研究表明,革兰氏阳性细菌(如金黄色葡萄球菌)通过协同激活CRs和TLR2受体,启动NOX2介导的ROS信号级联反应,促进导致染色质解聚和NETs释放[2,51];而革兰氏阴性菌(如大肠杆菌)则主要依赖TLR4途径诱导NETs形成[52]。通过查阅相关文献,本文总结了在畜禽动物特定感染模型中多种病原体诱导NETs形成的相关研究(表1)。
表1 畜禽动物模型中病原体诱导NETs形成的示例

Table 1 Examples of pathogen-induced NETs formation in livestock and poultry animal models

病原体类型
Pathogen type
具体病原体
Specific pathogen
宿主物种
Host species
疾病或病理模型
Disease or
pathological mode
文献
Reference
细菌
Bacteria
乳房链球菌Streptococcus uberis 绵羊 乳腺炎 [11]
沃纳氏葡萄球菌Staphylococcus warneri 山羊 乳腺炎体外模型 [8]
无乳链球菌Streptococcus agalactiae 乳腺炎 [53]
金黄色葡萄球菌Staphylococcus aureus 乳腺炎 [54]
大肠杆菌Escherichia coli 乳腺炎体外模型 [55]
耻垢分枝杆菌Mycobacterium smegmatis [56]
溶血性曼氏杆菌Mannheimia haemolytica 体外感染模型 [57]
链球菌Streptococcus suis 脑膜炎 [58]
胸膜肺炎放线杆菌Actinobacillus pleuropneumoniae 肺炎 [59]
支原体
Mycoplasma
无乳支原体Mycoplasma agalactiae 绵羊 乳腺炎 [60]
牛支原体Mycoplasma bovis 体外感染模型 [61]
鸡败血支原体Mycoplasma gallisepticum 鸡毒支原体病 [62]
十二指肠贾第鞭毛虫Giardia duodenalis 山羊 体外感染模型 [63]
肝片吸虫Fasciola hepatica 绵羊 肝吸虫病 [64]
弓形虫Toxoplasma gondii 绵羊和牛 弓形虫感染体外模型 [65]
犬新孢子虫Neospora caninum 山羊、牛 体外感染模型 [66-67]
艾美耳球虫Eimeria arloingi 山羊、牛 体外感染模型 [68-69]
奥氏奥斯特线虫Ostertagia ostertagi 感染体外模型 [9]
瘤胃吸虫Calicophoron daubneyi 体外感染模型 [70]
伊氏锥虫Trypanosoma evansi 骆驼 体外感染模型 [10]
病毒
Virus
呼吸道合胞病毒Respiratory syncytial virus 合胞病毒感染 [71]
甲型流感病毒Influenza A viruses 甲型流感病毒感染 [72]

2.2 代谢性疾病

目前,关于代谢性疾病诱导NETs形成的研究相对有限,且现有证据主要集中于反刍动物(主要是围产期奶牛),在单胃动物(如猪和家禽)中则鲜见相关报道。亚临床低血钙是高产奶牛在产犊后及泌乳初期常见的一种代谢性疾病,以血钙浓度持续低于正常生理水平(2 mmol/L)为主要特征。研究表明,亚临床低血钙奶牛可通过下调中性粒细胞内Ca2+浓度,导致线粒体发生损伤与ROS生成减少,最终抑制NETs的形成[73]。细胞内Ca2+浓度的变化是中性粒细胞激活的重要标志;在正常生理状态下,细胞受刺激后胞质Ca2+浓度会通过内质网等细胞内钙库的释放和/或细胞外Ca2+的内流而迅速升高[74]。然而,在亚临床低血钙奶牛中,由于钙释放激活钙调节蛋白1(calcium release-activated calcium modulator 1,ORAI1)基因的表达下调,中性粒细胞的钙摄取能力受损,导致其无法有效动员Ca2+,这可能是NETs形成受阻的重要原因[75]。酮病是围产期奶牛因能量代谢失衡所致的一种代谢性疾病,以血液中酮体(如β-羟丁酸、乙酰乙酸和丙酮)异常积累为主要表现,可显著增加奶牛罹患乳腺炎及其他传染病的风险[55]。体外研究表明,β-羟丁酸能够使大肠杆菌激活的奶牛中性粒细胞形成的NETs减少约10倍,并对其NETs相关杀菌活性产生类似程度的抑制[55]。另外,围产期奶牛由于脂质代谢活动加强而易发生能量负平衡,导致血液中游离脂肪酸(non-esterified fatty acids, NEFA)的浓度激增,而高浓度的NEFA会进一步参与机体氧化应激反应,并诱发失控的炎症反应[76]。NEFA通过激活核因子-κB(nuclear factor kappa-B,NF-κB)-NOD样受体热蛋白结构域相关蛋白3(NOD-like receptor thermal protein domain associated protein 3,NLRP3)-半胱天冬酶(cysteine-aspartic proteases,Caspase)1/4信号轴,促进Gasdermin D介导的孔道形成,同时伴随ROS含量升高,最终在体外诱导奶牛中性粒细胞释放NETs[77]。这些研究揭示了奶牛围产期代谢紊乱与NETs形成之间的复杂互作关系。

2.3 生殖受孕

在受孕过程中,精液在子宫内的沉积可激活中性粒细胞介导的免疫反应并诱导NETs的形成[78]。研究表明,牛精子与中性粒细胞在体外共培养15 min后即可观察到NETs的产生[79]。该过程依赖于NOX和PAD4的激活,并需要细胞内及细胞外Ca2+的协同流入[80]。值得注意的是,新鲜精液、冻融精液乃至单独的精浆均能诱导牛中性粒细胞形成NETs[78]。类似地,猪精子也可触发NETs形成,这不仅会损伤精子功能,还可导致NETs与胚胎发生纠缠[81],从而影响受孕结局。在生理状态下,精子诱导的NETs形成可能是一种进化上保守的防御机制,用于清除异常或缺陷精子[82]。然而,这一过程同时也会破坏精子质膜完整性、降低精子活力并削弱其受精能力,从而对繁殖效率产生负面影响[83]。另外,机体也形成相应的保护机制以维持生殖微环境的稳定。例如,牛输卵管可分泌多种活性因子[如前列腺素(E2)[84]、内皮素-1[85]和α1-酸性糖蛋白[86]],在保护精子免受NETs吞噬的同时,维持中性粒细胞对病原体的吞噬活性,从而有效遏制细菌传播[87],保障成功受孕。受孕过程中精液诱导NETs形成是影响动物繁殖效率的重要因素[88]

2.4 其他诱导因素

霉菌毒素是畜禽养殖中常见的饲料污染物,其中伏马菌素B1在鸡体内抑制NETs形成[89],而在牛中性粒细胞中通过NOX依赖途径在体外诱导NETs产生[90];玉米赤霉烯酮则通过诱导线粒体ROS爆发,激活细胞外信号调节激酶(extracellular signal-regulated kinase,ERK)和p38信号通路,从而促进NETs释放[91]。重金属污染如铅暴露可通过抑制鸡内质网Ca2+回流减少NETs形成,铝污染则通过影响猪硒蛋白信号通路抑制溶酶体ROS爆发及NETs释放,而硒在一定程度上可拮抗铅和铝的抑制作用[92-93]。此外,微量元素如铜、锌和硒在体外均能显著诱导奶牛NETs形成[94]。某些抗生素如恩诺沙星可通过促进革兰氏阴性菌释放LPS,进而增强牛中性粒细胞NETs的形成[95]。这些研究表明,多种外源物质均可有效诱导NETs的形成,为理解其在畜禽免疫调控与健康中的作用提供了理论依据。

3 NETs在畜禽健康中的作用

3.1 病原体捕获和清除

NETs通过其特有的DNA-蛋白质复合网状结构,形成高效的物理捕获屏障,实现对病原体的快速固定和滞留。从结构基础来看,NETs由DNA纤维和球形蛋白组装形成的特征性球形功能区可物理性限制病原体运动,同时纤维上密集分布的抗菌蛋白(如MPO、NE等活性迅速提升)形成强效杀菌微环境[1,96]。在体外病原刺激下,经扫描电镜观察可见,牛中性粒细胞在受到十二指肠贾第鞭毛虫滋养体或犬新孢子虫速殖子体外刺激后,均能释放NETs,形成典型的网状纤维结构,并有效捕获与包裹病原体[67,97]。绵羊体内NETs也通过释放含抗菌蛋白的DNA复合物可高效捕获乳房链球菌[11]。有趣的是,牛、羊中性粒细胞在响应弓形虫速殖子时表现出显著的种属差异[65]:牛源中性粒细胞主要依赖高活性MPO实现对病原体的高效杀伤,而羊源中性粒细胞则主要通过形成NETs对虫体进行物理禁锢,限制其移动。类似地,阿氏艾美耳球虫可诱导山羊NETs形成并被其捕获,但NETs仅具物理束缚作用,无法显著影响虫体存活率[68]。值得注意的是,链球菌和支原体可分别通过分泌核酸酶A,降解猪源与牛源NETs的DNA骨架,进而逃逸NETs介导的免疫捕获作用[98-99]。金黄色葡萄球菌也可通过调控Ca2+通道,改变低血钙症奶牛外周血中性粒细胞内Ca2+浓度进而诱导自噬体形成并阻断自噬通量,最终实现免疫逃逸[99]。因此,NETs通过捕获病原体为宿主构筑先天防御屏障,但其效能常被病原体的逃逸机制所削弱,而未来针对逃逸因子的靶向中和策略或NETs稳定性的增强手段,有望成为防控畜禽疫病的新方向。

3.2 加剧组织损伤

NETs在免疫防御中发挥重要作用,但其过度或持续存在可能导致细胞和组织的炎症损伤。过量的NETs通过其细胞毒性组分(如组蛋白和NE)破坏细胞膜完整性及细胞间基质蛋白,导致内皮细胞和上皮细胞的连接结构损伤,从而加剧组织病理损伤[100-101]。在以猪为损伤模型的研究中发现,缺血再灌注通过诱导NETs浸润及PAD释放,催化纤维蛋白原等血浆蛋白瓜氨酸化,加重组织损伤[102];而清除NETs可改善吸入性肺损伤供肺的功能与形态,表明靶向NETs具有治疗潜力[103]。在畜禽健康方面,关于NETs介导的炎性损伤研究主要聚焦于奶牛乳腺炎模型,特别是NETs对乳腺上皮细胞的损伤机制及其分子通路[104-105]。NETs的主要组成成分组蛋白通过激活Caspase-1、NLRP3和Caspase-3等凋亡蛋白或炎症小体,诱导乳腺上皮细胞发生焦亡、凋亡和坏死,从而损伤乳腺上皮屏障[106]。NETs在奶牛子宫内膜炎发病过程中通过高迁移率族蛋白B1(high mobility group protein,HMGB1)/NLRP3/Caspase-1信号通路诱导子宫内膜上皮细胞焦亡,导致组织炎症和损伤;而抑制NETs形成可显著缓解上述病理变化[107]。此外,研究还发现,NETs的形成是母体营养不良诱发宫内生长发育受限绵羊胎儿肝脏损伤的一个新机制[12]。这些发现表明,NETs作为重要的免疫效应机制,在其调控失衡时会转化为关键致病介质,加剧组织损伤进程。

4 营养调控在畜禽NETs形成中的作用

营养调控对畜禽NETs的形成表现出双向调节作用。一方面,槲皮素和山奈酚可以降低ROS的形成,从而抑制NETs的形成并缓解其对山羊精子的损伤[108-109];油酸[110]和丁酸钠[14]则分别在体外通过抑制自噬通量和中性粒细胞自噬来减少奶牛中性粒细胞形成NETs。另一方面,在抗感染过程中,槲皮素可通过增强ROS介导的杀菌功能促进NETs释放[111];女贞子活性物质(齐墩果酸和红景天苷)[112]及烟酸[13]也可通过不同机制在体外诱导奶牛中性粒细胞形成NETs,增强病原体清除能力。这表明营养对NETs的调控具有多样性,既可通过抗氧化和抑制自噬等途径抑制过度炎症损伤,也可在免疫防御中增强NETs的抗菌功能。目前,关于营养调控在畜禽NETs中的作用研究仍处于初步阶段,相关报道多局限于体外试验,亟待更多体内研究进一步验证其调控机制与应用潜力。

5 小结

NETs作为先天免疫防御的重要组成部分,其适度形成对抵抗病原微生物感染至关重要,而过度激活则可能加剧组织炎症和损伤。在畜禽动物中,NETs最初被认为参与对抗各类病原体的免疫反应,而近年研究进一步揭示其与乳腺炎、子宫内膜炎等疾病相关的组织损伤机制密切相关。目前,一些植物提取物和脂肪酸等营养活性物质已在体外被证实可调控NETs的形成,但相关研究仍存在分子机制解析不足、NETs动态平衡调控研究缺乏以及实际生产应用效果待验证等局限。值得注意的是,过度抑制NETs可能削弱先天免疫防御功能,反而增加感染风险,因此在养殖生产中需权衡其调控策略。未来,深入探究营养干预对NETs形成与功能的调控机制,不仅可为自身免疫性疾病的防治提供新思路,也将为畜禽健康养殖提供理论依据。然而,NETs作为一种新兴的免疫机制,其调控网络及生理病理意义仍有待进一步阐明,相关研究尚处于起步阶段,需更多系统性探索以推动其在畜牧及兽医领域的应用。
[1]
BRINKMANN V, REICHARD U, GOOSMANN C, et al. Neutrophil extracellular traps kill bacteria[J]. Science, 2004, 303(5663):1532-1535.

DOI PMID

[2]
FUCHS T A, ABED U, GOOSMANN C, et al. Novel cell death program leads to neutrophil extracellular traps[J]. The Journal of Cell Biology, 2007, 176(2):231-241.

DOI

[3]
杨康洁, 芦永良, 鄂维建. 中性粒细胞胞外诱捕网与适应性免疫细胞失衡关系的研究进展[J]. 现代免疫学, 2025, 45(2):230-235,242.

YANG K J, LU Y L, E W J. Research progress on the relationship between neutrophil extracellular trap and adaptive immune cell imbalance[J]. Current Immunology, 2025, 45(2):230-235,242. (in Chinese)

[4]
PAPAYANNOPOULOS V. Neutrophil extracellular traps in immunity and disease[J]. Nature Reviews Immunology, 2018, 18(2):134-147.

DOI PMID

[5]
THIAM H R, WONG S L, WAGNER D D, et al. Cellular mechanisms of NETosis[J]. Annual Review of Cell and Developmental Biology, 2020, 36:191-218.

DOI

[6]
CAO C Y, CHEN N X, ZHU H Q, et al. Selenium ameliorates aluminum poisoning-induced impaired production of neutrophil extracellular traps in chicken[J]. Biological Trace Element Research, 2025, 203(8):4318-4325.

DOI

[7]
BONILLA M C, QUIROS O N, WENDT M, et al. New insights into neutrophil extracellular trap (NETs) formation from porcine neutrophils in response to bacterial infections[J]. International Journal of Molecular Sciences, 2022, 23(16):8953.

DOI

[8]
CALDEIRA J L A, COSTA D G, POLVEIRO R C, et al. Short communication:goat mastitis and the formation of neutrophil extracellular traps (NETs)[J]. Veterinary Immunology and Immunopathology, 2024, 274:110793.

DOI

[9]
MENDEZ J, SUN D L, TUO W B, et al. Bovine neutrophils form extracellular traps in response to the gastrointestinal parasite Ostertagia ostertagi[J]. Scientific Reports, 2018, 8(1):17598.

DOI

[10]
HUSSEN J, AL-JABR O A, ALKUWAYTI M A, et al. A flow cytometry study of the binding and stimulation potential of inactivated Trypanosoma evansi toward dromedary camel leukocytes[J]. Pathogens, 2023, 13(1):21.

DOI

[11]
PISANU S, CUBEDDU T, PAGNOZZI D, et al. Neutrophil extracellular traps in sheep mastitis[J]. Veterinary Research, 2015, 46(1):59.

DOI

[12]
ZI Y, QIN Y L, MA C, et al. Transcriptome analysis reveals hepatic disordered lipid metabolism,lipotoxic injury,and abnormal development in IUGR sheep fetuses due to maternal undernutrition during late pregnancy[J]. Theriogenology, 2024, 226:350-362.

DOI

[13]
CARRETTA M D, CREUTZBURG P, BORQUEZ K, et al. Hydroxycarboxylic acid receptor 2 (HCA2) agonists induce NET formation and MMP-9 release from bovine polymorphonuclear leukocytes[J]. Developmental and Comparative Immunology, 2023, 139:104562.

DOI

[14]
LI Y H, LIU J X, CUI Y Y, et al. Sodium butyrate attenuates bovine mammary epithelial cell injury by inhibiting the formation of neutrophil extracellular traps[J]. International Immunopharmacology, 2022, 110:109009.

DOI

[15]
PAAPE M J, BANNERMAN D D, ZHAO X, et al. The bovine neutrophil:structure and function in blood and milk[J]. Veterinary Research, 2003, 34(5):597-627.

DOI

[16]
HIDALGO A, LIBBY P, SOEHNLEIN O, et al. Neutrophil extracellular traps:from physiology to pathology[J]. Cardiovascular Research, 2022, 118(13):2737-2753.

DOI

[17]
MA Y X, WEI J L, HE W S, et al. Neutrophil extracellular traps in cancer[J]. MedComm, 2024, 5(8):e647.

DOI PMID

[18]
BRAVO-BARRERA J, KOURILOVITCH M, GALARZA-MALDONADO C. Neutrophil extracellular traps,antiphospholipid antibodies and treatment[J]. Antibodies, 2017, 6(1):4.

DOI

[19]
HAMAM H J, KHAN M A, PALANIYAR N. Histone acetylation promotes neutrophil extracellular trap formation[J]. Biomolecules, 2019, 9(1):32.

DOI

[20]
HANN J, BUEB J L, TOLLE F, et al. Calcium signaling and regulation of neutrophil functions:still a long way to go[J]. Journal of Leukocyte Biology, 2020, 107(2):285-297.

DOI

[21]
PACLET M H, LAURANS S, DUPRÉ-CROCHET S. Regulation of neutrophil NADPH oxidase,NOX2:a crucial effector in neutrophil phenotype and function[J]. Frontiers in Cell and Developmental Biology, 2022, 10:945749.

DOI

[22]
HOOK J S, CAO M, POTERA R M, et al. Nox2 regulates platelet activation and NET formation in the lung[J]. Frontiers in Immunology, 2019, 10:1472.

DOI

[23]
ZHU D, LU Y, GUI L, et al. Self-assembling, pH-responsive nanoflowers for inhibiting PAD4 and neutrophil extracellular trap formation and improving the tumor immune microenvironment[J]. Acta Pharmaceutica Sinica B, 2022, 12(5):2592-2608.

DOI PMID

[24]
DOUDA D N, KHAN M A, GRASEMANN H, et al. SK3 channel and mitochondrial ROS mediate NADPH oxidase-independent NETosis induced by calcium influx[J]. Proceedings of the National Academy of Sciences of the United States of America, 2015, 112(9):2817-2822.

DOI PMID

[25]
YOUSEFI S, MIHALACHE C, KOZLOWSKI E, et al. Viable neutrophils release mitochondrial DNA to form neutrophil extracellular traps[J]. Cell Death and Differentiation, 2009, 16(11):1438-1444.

DOI PMID

[26]
DELGADO-RIZO V, MARTÍNEZ-GUZMÁN M A, IÑIGUEZ-GUTIERREZ L, et al. Neutrophil extracellular traps and its implications in inflammation:an overview[J]. Frontiers in Immunology, 2017, 8:81.

[27]
RONCHETTI L, BOUBAKER N S, BARBA M, et al. Neutrophil extracellular traps in cancer:not only catching microbes[J]. Journal of Experimental & Clinical Cancer Research, 2021, 40(1):231.

[28]
PENG F, XIE J N, LIU H M, et al. Shifting focus from bacteria to host neutrophil extracellular traps of biodegradable pure Zn to combat implant centered infection[J]. Bioactive Materials, 2023, 21:436-449.

DOI PMID

[29]
LI R H L, NG G, TABLIN F. Lipopolysaccharide-induced neutrophil extracellular trap formation in canine neutrophils is dependent on histone H3 citrullination by peptidylarginine deiminase[J]. Veterinary Immunology and Immunopathology, 2017,193/194:29-37.

[30]
HONDA M, KUBES P. Neutrophils and neutrophil extracellular traps in the liver and gastrointestinal system[J]. Nature Reviews Gastroenterology & Hepatology, 2018, 15(4):206-221.

[31]
DABROWSKA D, JABŁOŃSKA E, GARLEY M, et al. New aspects of the biology of neutrophil extracellular traps[J]. Scandinavian Journal of Immunology, 2016, 84(6):317-322.

DOI PMID

[32]
XUAN N X, ZHAO J, KANG Z Y, et al. Neutrophil extracellular traps and their implications in airway inflammatory diseases[J]. Frontiers in Medicine, 2023, 10:1331000.

DOI

[33]
姜慧华, 李宁, 徐磊, 等. 中性粒细胞胞外诱捕网在病原感染中的作用研究进展[J]. 畜牧兽医学报, 2023, 54(3):889-899.

DOI

JIANG H H, LI N, XU L, et al. Research progress on the role of neutrophil extracellular traps in pathogenic infection[J]. Acta Veterinaria et Zootechnica Sinica, 2023, 54(3):889-899. (in Chinese)

DOI

[34]
KONG Y, HE G Q, ZHANG X L, et al. The role of neutrophil extracellular traps in lipopolysaccharide-induced depression-like behaviors in mice[J]. Brain Sciences, 2021, 11(11):1514.

DOI

[35]
黄嘉祺, 方金花, 吴芝伟, 等. 脂磷壁酸诱导稳定黏附于ICAM-1上的中性粒细胞胞外诱捕网形成[J]. 生物医学工程学杂志, 2024, 41(2):304-312.

HUANG J Q, FANG J H, WU Z W, et al. Neutrophil extracellular traps extrusion from neutrophils stably adhered to ICAM-1 by lipoteichoic acid stimulation[J]. Journal of biomedical engineering, 2024, 41(2):304-312. (in Chinese)

[36]
FLOYD M, WINN M, CULLEN C, et al. Swimming motility mediates the formation of neutrophil extracellular traps induced by flagellated Pseudomonas aeruginosa[J]. PLoS Pathogens, 2016, 12(11):e1005987.

DOI

[37]
SCHNEIDER A E, SÁNDOR N, KÁRPÁTI É, et al. Complement factor H modulates the activation of human neutrophil granulocytes and the generation of neutrophil extracellular traps[J]. Molecular Immunology, 2016, 72:37-48.

DOI PMID

[38]
ZAWROTNIAK M, BOCHENSKA O, KARKOWSKA-KULETA J, et al. Aspartic proteases and major cell wall components in Candida albicans trigger the release of neutrophil extracellular traps[J]. Frontiers in Cellular and Infection Microbiology, 2017, 7:414.

DOI

[39]
ZAWROTNIAK M, WOJTALIK K, RAPALA-KOZIK M. Farnesol,a quorum-sensing molecule of Candida albicans triggers the release of neutrophil extracellular traps[J]. Cells, 2019, 8(12):1611.

DOI

[40]
REIS A P C, CELESTRINO G A, IGOA M V B, et al. The dermatophyte trichophyton rubrum induces neutrophil extracellular traps release by human neutrophils[J]. Journal of Fungi, 2022, 8(2):147.

DOI

[41]
URBAN C F, REICHARD U, BRINKMANN V, et al. Neutrophil extracellular traps capture and kill Candida albicans yeast and hyphal forms[J]. Cellular Microbiology, 2006, 8(4):668-676.

DOI

[42]
ORTMANN W, SUCH A, CICHON I, et al. Large extracellular vesicle (EV) and neutrophil extracellular trap (NET) interaction captured in vivo during systemic inflammation[J]. Scientific Reports, 2024, 14(1):4680.

DOI

[43]
RABINOVITCH M. NETs activate pulmonary arterial endothelial cells[J]. Arteriosclerosis,Thrombosis,and Vascular Biology, 2016, 36(10):2035-2037.

DOI

[44]
RAFTERY M J, LALWANI P, KRAUTKRÄMER E, et al. β2 integrin mediates hantavirus-induced release of neutrophil extracellular traps[J]. The Journal of Experimental Medicine, 2014, 211(7):1485-1497.

DOI PMID

[45]
BREDA L C D, DE SOUZA BREDA C N, DE ALMEIDA J R F, et al. Fonsecaeapedrosoi conidia and hyphae activate neutrophils distinctly:requirement of TLR-2 and TLR-4 in neutrophil effector functions[J]. Frontiers in Immunology, 2020, 11:540064.

DOI

[46]
TONG M, SMITH A H, ABRAHAMS V M. Activated neutrophils propagate fetal membrane inflammation and weakening through ERK and neutrophil extracellular Trap-INDUCED TLR-9 signaling[J]. The Journal of Immunology, 2021, 206(5):1039-1045.

DOI

[47]
ALYAMI H M, FINOTI L S, TEIXEIRA H S, et al. Role of NOD1/NOD2 receptors in Fusobacterium nucleatum mediated NETosis[J]. Microbial Pathogenesis, 2019, 131:53-64.

DOI

[48]
LI K, UNDERHILL D M. C-Type lectin receptors in phagocytosis[J]. Current Topics in Microbiology and Immunology, 2020, 429:1-18.

[49]
PALMER L J, DAMGAARD C, HOLMSTRUP P, et al. Influence of complement on neutrophil extracellular trap release induced by bacteria[J]. Journal of Periodontal Research, 2016, 51(1):70-76.

DOI PMID

[50]
BRYZEK D, CIASTON I, DOBOSZ E, et al. Triggering NETosis via protease-activated receptor (PAR)-2 signaling as a mechanism of hijacking neutrophils function for pathogen benefits[J]. PLoS Pathogens, 2019, 15(5):e1007773.

DOI

[51]
LIPINSKA-GEDIGA M. Neutrophils,NETs,NETosis-old or new factors in sepsis and septic shock?[J]. Anaesthesiology Intensive Therapy, 2017, 49(3):235-240.

DOI

[52]
HU N, WESTRA J, KALLENBERG C G M. Dysregulated neutrophil-endothelial interaction in antineutrophil cytoplasmic autoantibody (ANCA)-associated vasculitides:implications for pathogenesis and disease intervention[J]. Autoimmunity Reviews, 2011, 10(9):536-543.

DOI

[53]
MA F, YANG S F, WANG G Y, et al. Effect of multiplicity of infection on the evasion of neutrophil killing by Streptococcus agalactiae isolated from clinical mastitis bovine[J]. Veterinary Microbiology, 2022, 270:109450.

DOI

[54]
REINHARDT T A, SACCO R E, NONNECKE B J, et al. Bovine milk proteome:quantitative changes in normal milk exosomes,milk fat globule membranes and whey proteomes resulting from Staphylococcus aureus mastitis[J]. Journal of Proteomics, 2013, 82:141-154.

DOI

[55]
GRINBERG N, ELAZAR S, ROSENSHINE I, et al. Beta-hydroxybutyrate abrogates formation of bovine neutrophil extracellular traps and bactericidal activity against mammary pathogenic Escherichia coli[J]. Infection and Immunity, 2008, 76(6):2802-2807.

DOI

[56]
臧鑫鑫, 党光辉, 王忠星, 等. 耻垢分枝杆菌诱导中性粒细胞胞外诱捕网形成的研究[J]. 中国预防兽医学报, 2019, 41(11):1154-1158.

ZANG X X, DANG G H, WANG Z X, et al. Study on the formation of neutrophil extracellular traps induced by Mycobacterium smegmatis[J]. Chinese Journal of Preventive Veterinary Medicine, 2019, 41(11):1154-1158. (in Chinese)

[57]
AULIK N A, HELLENBRAND K M, KLOS H, et al. Mannheimia haemolytica and its leukotoxin cause neutrophil extracellular trap formation by bovine neutrophils[J]. Infection and Immunity, 2010, 78(11):4454-4466.

DOI PMID

[58]
MEURER M, ÖHLMANN S, BONILLA M C, et al. Role of bacterial and host DNases on host-pathogen interaction during Streptococcus suis meningitis[J]. International Journal of Molecular Sciences, 2020, 21(15):5289.

DOI

[59]
DE BUHR N, BONILLA M C, PFEIFFER J, et al. Degraded neutrophil extracellular traps promote the growth of Actinobacillus pleuropneumoniae[J]. Cell Death & Disease, 2019, 10(9):657.

[60]
CACCIOTTO C, CUBEDDU T, ADDIS M F, et al. Mycoplasma lipoproteins are major determinants of neutrophil extracellular trap formation[J]. Cellular Microbiology, 2016, 18(12):1751-1762.

DOI PMID

[61]
MITIKU F, HARTLEY C A, SANSOM F M, et al. The major membrane nuclease MnuA degrades neutrophil extracellular traps induced by Mycoplasma bovis[J]. Veterinary Microbiology, 2018, 218:13-19.

DOI

[62]
WANG S, NIU D, HU J Q, et al. Exploiting an evolutionary constraint:targeting TatD nuclease with chrysosplenol D disrupts Mycoplasma gallisepticum infection[J]. International Journal of Biological Macromolecules, 2025, 321(Pt 3):146394.

DOI

[63]
JIANG X, LI Q Y, HUANG R S, et al. Giardia duodenalis triggered neutrophil extracellular traps in goats[J]. Immunobiology, 2025, 230(3):152894.

DOI

[64]
MUÑOZ-CARO T, GÓMEZ-CERUTI M, SILVA L M R, et al. Fasciola hepatica soluble antigens (FhAg) induce ovine PMN innate immune reactions and NET formation in vitro and in vivo[J]. Veterinary Research, 2023, 54(1):105.

DOI

[65]
YILDIZ K, GOKPINAR S, GAZYAGCI A N, et al. Role of NETs in the difference in host susceptibility to Toxoplasma gondii between sheep and cattle[J]. Veterinary Immunology and Immunopathology, 2017, 189:1-10.

DOI

[66]
VILLAGRA-BLANCO R, SILVA L M R, GÄRTNER U, et al. Molecular analyses on Neospora caninum-triggered NETosis in the caprine system[J]. Developmental and Comparative Immunology, 2017, 72:119-127.

DOI

[67]
VILLAGRA-BLANCO R, SILVA L M R, MUÑOZ-CARO T, et al. Bovine polymorphonuclear neutrophils cast neutrophil extracellular traps against the abortive parasite neospora caninum[J]. Frontiers in Immunology, 2017, 8:606.

DOI

[68]
SILVA L M R, CARO T M, GERSTBERGER R, et al. The apicomplexan parasite Eimeria arloingi induces caprine neutrophil extracellular traps[J]. Parasitology Research, 2014, 113(8):2797-2807.

DOI

[69]
MUÑOZ-CARO T, MENA HUERTAS S J, CONEJEROS I, et al. Eimeria bovis-triggered neutrophil extracellular trap formation is CD11b-,ERK 1/2-,p38 MAP kinase- and SOCE-dependent[J]. Veterinary Research, 2015, 46:23.

DOI

[70]
SILVA L M R, LÓPEZ-OSORIO S, PEIXOTO R, et al. Cellular immune responses of bovine polymorphonuclear neutrophils to Calicophoron daubneyi[J]. Frontiers in Immunology, 2025, 16:1515419.

DOI

[71]
MUTUA V, CAVALLO F, GERSHWIN L J. Neutrophil extracellular traps (NETs) in a randomized controlled trial of a combination of antiviral and nonsteroidal anti-inflammatory treatment in a bovine model of respiratory syncytial virus infection[J]. Veterinary Immunology and Immunopathology, 2021, 241:110323.

DOI PMID

[72]
LASSNIG S, HENNIG-PAUKA I, BONILLA M C, et al. Impact of bronchoalveolar lavage from influenza A virus diseased pigs on neutrophil functions and growth of co-infecting pathogenic bacteria[J]. Frontiers in Immunology, 2024, 15:1325269.

DOI

[73]
ZHANG B B, MA X R, LOOR J J, et al. Role of ORAI calcium release-activated calcium modulator 1 (ORAI1) on neutrophil extracellular trap formation in dairy cows with subclinical hypocalcemia[J]. Journal of Dairy Science, 2022, 105(4):3394-3404.

DOI PMID

[74]
IMMLER R, SIMON S I, SPERANDIO M. Calcium signalling and related ion channels in neutrophil recruitment and function[J]. European Journal of Clinical Investigation, 2018, 48(S2):e12964.

DOI

[75]
ZHANG B B, GUO H, YANG W, et al. Effects of ORAI calcium release-activated calcium modulator 1 (ORAI1) on neutrophil activity in dairy cows with subclinical hypocalcemia1[J]. Journal of Animal Science, 2019, 97(8):3326-3336.

DOI PMID

[76]
SORDILLO L M, RAPHAEL W. Significance of metabolic stress,lipid mobilization,and inflammation on transition cow disorders[J]. The Veterinary Clinics of North America.Food Animal Practice, 2013, 29(2):267-278.

[77]
谢磊. 奶牛不同生理阶段和NEFA对中性粒细胞胞外诱捕网形成的影响[D]. 硕士学位论文. 杨凌: 西北农林科技大学, 2022.

XIE L. Effects of different physiological stages and NEFA on the formation of neutrophil extracellular traps in dairy cows[D]. Master’s Thesis. Yangling: Northwest A&F University, 2022. (in Chinese)

[78]
FICHTNER T, KOTARSKI F, HERMOSILLA C, et al. Semen extender and seminal plasma alter the extent of neutrophil extracellular traps (NET) formation in cattle[J]. Theriogenology, 2021, 160:72-80.

DOI PMID

[79]
RIVERA-CONCHA R, LEÓN M, PRADO-SANHUEZA A, et al. Cytotoxic oxidative stress effects of neutrophil extracellular traps’ components on cattle spermatozoa[J]. Antioxidants, 2024, 13(6):733.

DOI

[80]
FICHTNER T, KOTARSKI F, GÄRTNER U, et al. Bovine sperm samples induce different NET phenotypes in a NADPH oxidase-,PAD4-,and Ca2+-dependent process[J]. Biology of Reproduction, 2020, 102(4):902-914.

DOI

[81]
WEI Z K, YU T T, WANG J J, et al. Swine sperm induces neutrophil extracellular traps that entangle sperm and embryos[J]. Reproduction, 2020, 160(2):217-225.

DOI

[82]
WRENZYCKI C. Interaction of sperm cells with the female reproductive tract in cattle:focus on neutrophil extracellular trap formation[J]. Animal Reproduction Science, 2022, 246:107056.

DOI

[83]
ZAMBRANO F, NAMUNCURA C, URIBE P, et al. Swine spermatozoa trigger aggregated neutrophil extracellular traps leading to adverse effects on sperm function[J]. Journal of Reproductive Immunology, 2021, 146:103339.

DOI

[84]
MAREY M A, LIU J H, KOWSAR R, et al. Bovine oviduct epithelial cells downregulate phagocytosis of sperm by neutrophils:prostaglandin E2 as a major physiological regulator[J]. Reproduction, 2014, 147(2):211-219.

DOI

[85]
MAREY M A, YOUSEF M S, LIU J H, et al. Endothelin-1 downregulates sperm phagocytosis by neutrophils in vitro:a physiological implication in bovine oviduct immunity[J]. Journal of Reproduction and Development, 2016, 62(2):151-157.

DOI

[86]
LIU J H, MAREY M A, KOWSAR R, et al. An acute-phase protein as a regulator of sperm survival in the bovine oviduct:alpha 1-acid-glycoprotein impairs neutrophil phagocytosis of sperm in vitro[J]. Journal of Reproduction and Development, 2014, 60(5):342-348.

DOI

[87]
MAREY M A, MATSUKAWA H, SASAKI M, et al. Bovine oviduct epithelial cells suppress the phagocytic activity of neutrophils towards sperm but not for bacteria in vitro:immunofluorescence and electron microscopic observations[J]. Histology and Histopathology, 2020, 35(6):589-597.

[88]
RIVERA-CONCHA R, MOYA C, LEÓN M, et al. Effect of different sperm populations on neutrophils extracellular traps (NETs) formation in cattle[J]. Research in Veterinary Science, 2023, 164:105028.

DOI

[89]
ZHU H Q, YU Q F, OUYANG H M, et al. Antagonistic effect of selenium on fumonisin B1 promotes neutrophil extracellular traps formation in chicken neutrophils[J]. Journal of Agricultural and Food Chemistry, 2022, 70(19):5911-5920.

DOI PMID

[90]
WANG J J, LIU Z Y, HAN Z, et al. Fumonisin B1 triggers the formation of bovine neutrophil extracellular traps[J]. Toxicology Letters, 2020, 332:140-145.

DOI

[91]
WANG J J, WEI Z K, HAN Z, et al. Zearalenone induces estrogen-receptor-independent neutrophil extracellular trap release in vitro[J]. Journal of Agricultural and Food Chemistry, 2019, 67(16):4588-4594.

DOI

[92]
YIN K, YANG Z J, GONG Y Z, et al. The antagonistic effect of Se on the Pb-weakening formation of neutrophil extracellular traps in chicken neutrophils[J]. Ecotoxicology and Environmental Safety, 2019, 173:225-234.

DOI PMID

[93]
ZHU H Q, CHEN S, LI R B, et al. Selenium-rich yeast counteracts the inhibitory effect of nanoaluminum on the formation of porcine neutrophil extracellular traps[J]. Research in Veterinary Science, 2023, 161:138-144.

DOI PMID

[94]
ZHOU X C, WANG H, LIAN S, et al. Effect of copper,zinc,and selenium on the formation of bovine neutrophil extracellular traps[J]. Biological Trace Element Research, 2021, 199(9):3312-3318.

DOI

[95]
JERJOMICEVA N, SERI H, VÖLLGER L, et al. Enrofloxacin enhances the formation of neutrophil extracellular traps in bovine granulocytes[J]. Journal of Innate Immunity, 2014, 6(5):706-712.

DOI PMID

[96]
LI S, WANG H, SHAO Q X. The central role of neutrophil extracellular traps (NETs) and by-products in COVID-19 related pulmonary thrombosis[J]. Immunity Inflammation and Disease, 2023, 11(8):e949.

DOI PMID

[97]
LI T Y, SUN Y P, WANG X, et al. Giardia duodenalis trophozoites triggered bovine neutrophil extracellular traps formation dependent on P2X1 receptor and PAD4 in vitro[J]. Veterinary Parasitology, 2022, 312:109841.

DOI

[98]
DE BUHR N, NEUMANN A, JERJOMICEVA N, et al. Streptococcus suis DNase SsnA contributes to degradation of neutrophil extracellular traps (NETs) and evasion of NET-mediated antimicrobial activity[J]. Microbiology, 2014, 160(2):385-395.

DOI

[99]
吕鑫泉. ORAI1/LC3调控低钙血症奶牛中性粒细胞介导金黄色葡萄球菌免疫逃逸作用[D]. 硕士学位论文. 大庆: 黑龙江八一农垦大学, 2024.

LV X Q. ORAI1/LC3-mediated regulation of Staphylococcus aureus immune escape by neutrophils in hypocalcemic dairy cows[D]. Master’s Thesis. Daqing: Heilongjiang Bayi Agricultural University, 2024. (in Chinese)

[100]
PIETERSE E, ROTHER N, GARSEN M, et al. Neutrophil extracellular traps drive endothelial-to-mesenchymal transition[J]. Arteriosclerosis,Thrombosis,and Vascular Biology, 2017, 37(7):1371-1379.

DOI

[101]
SAFFARZADEH M, JUENEMANN C, QUEISSER M A, et al. Neutrophil extracellular traps directly induce epithelial and endothelial cell death:a predominant role of histones[J]. PLoS One, 2012, 7(2):e32366.

DOI

[102]
ZOLLET V, ARENAS HOYOS I, HIRSIGER S, et al. Neutrophil extracellular traps and citrullinated fibrinogen contribute to injury in a porcine model of limb ischemia and reperfusion[J]. Frontiers in Immunology, 2024, 15:1436926.

DOI

[103]
MITTENDORFER M, PIERRE L, HUZEVKA T, et al. Restoring discarded porcine lungs by ex vivo removal of neutrophil extracellular traps[J]. The Journal of Heart and Lung Transplantation, 2024, 43(12):1919-1929.

DOI

[104]
WEI Z K, WANG J J, WANG Y N, et al. Effects of neutrophil extracellular traps on bovine mammary epithelial cells in vitro[J]. Frontiers in Immunology, 2019, 10:1003.

DOI

[105]
JIANG L Y, SUN H Z, GU F F, et al. Blood neutrophil extracellular traps:a novel target for the assessment of mammary health in transition dairy cows[J]. Journal of Animal Science and Biotechnology, 2023, 14(3):1068-1079.

[106]
魏正凯. 中性粒细胞胞外诱捕网对奶牛乳腺组织的免疫损伤作用及机制[D]. 博士学位论文. 长春: 吉林大学, 2019.

WEI Z K. Immunopathological effects and mechanisms of neutrophil extracellular traps on bovine mammary tissue[D]. Ph.D. Thesis. Changchun: Jilin University, 2019. (in Chinese)

[107]
沈文祥. 中性粒细胞胞外诱捕网介导奶牛子宫内膜炎症和组织损伤的机制研究[D]. 博士学位论文. 杨凌: 西北农林科技大学, 2023.

SHEN W X. Study of mechanisms of neutrophil extracellular trap-mediated endometrial inflammation and tissue damage in dairy cows[D]. Ph.D.Thesis. Yangling: Northwest A&F University, 2023. (in Chinese)

[108]
WEI Z K, HONG H R, LIU W, et al. Quercetin protects goat sperm motility by inhibiting neutrophil extracellular traps and maintaining plasma membrane and acrosome integrity[J]. Veterinary Sciences, 2024, 11(11):553.

DOI

[109]
洪鸿荣. 山奈酚对山羊中性粒细胞损伤精子的保护作用的初步研究[D]. 硕士学位论文. 佛山: 佛山科学技术学院, 2024.

HONG H R. Preliminary study on the protective effect of kaempferol on neutrophil-induced sperm damage in goats[D]. Master’s Thesis. Foshan: Foshan University, 2024. (in Chinese)

[110]
FENG X C, SONG Y X, SUN Z A, et al. Palmitic acid hinders extracellular traps of neutrophil from postpartum dairy cow in vitro[J]. Journal of Dairy Science, 2022, 105(10):8286-8297.

DOI

[111]
DISBANCHONG P, PUNMANEE W, SRITHANASUWAN A, et al. Immunomodulatory effects of herbal compounds quercetin and curcumin on cellular and molecular functions of bovine-milk-isolated neutrophils toward Streptococcus agalactiae infection[J]. Animals, 2021, 11(11):3286.

DOI

[112]
冯献程. 围产期奶牛能量代谢和免疫状态变化及女贞子的调节作用[D]. 博士学位论文. 长春: 吉林大学, 2023.

FENG X C. Changes of energy metabolism and immune status in peripartal cows and their regulation of Ligustrum lucidum[D]. Ph.D.Thesis. Changchun: Jilin University, 2023. (in Chinese)

文章导航

/