综述

几种常见脂肪酸对动物肠道健康的影响及其在动物生产中的应用研究进展

  • 李航 , 1 ,
  • 刘杰 1, 2 ,
  • 刘祝英 , 3, * ,
  • 伍树松 1
展开
  • 1 湖南农业大学动物科学技术学院, 长沙 410128
  • 2 湘中幼儿师范高等专科学校, 邵阳 422000
  • 3 湖南生物机电职业技术学院, 长沙 410128
* 刘祝英,讲师,E-mail:

李 航(2000—),男,湖南郴州人,硕士研究生,从事生猪绿色健康养殖研究工作。E-mail:

收稿日期: 2025-06-25

  网络出版日期: 2025-12-13

基金资助

国家重点研发计划项目(2023YFD1302300)

Research Progress on Effects of Several Common Fatty Acids on Animal Intestinal Health and Their Application in Animal Production

  • LI Hang , 1 ,
  • LIU Jie 1, 2 ,
  • LIU Zhuying , 3, * ,
  • WU Shusong 1
Expand
  • 1 College of Animal Science and Technology, Hunan Agricultural University, Changsha 410128, China
  • 2 Xiangzhong Normal for Preschool Education, Shaoyang 422000, China
  • 3 Hunan Biological Electromechanical Vocational Technical College, Changsha 410128, China
* lecturer, E-mail:

Received date: 2025-06-25

  Online published: 2025-12-13

摘要

短链脂肪酸(SCFA)、中链脂肪酸(MCFA)和多不饱和脂肪酸(PUFA)是常见的天然营养素,在调节动物体肠道健康方面表现出良好的功效。本文综述了常见的功能性脂肪酸SCFA、MCFA和PUFA,并从肠道细胞和组织形态、免疫功能及微生物等层面探讨了这几种常见脂肪酸对动物肠道健康的调控作用,以期为这几种常见脂肪酸在动物肠道健康和动物生产中的应用提供参考。

本文引用格式

李航 , 刘杰 , 刘祝英 , 伍树松 . 几种常见脂肪酸对动物肠道健康的影响及其在动物生产中的应用研究进展[J]. 动物营养学报, 2025 , 37(12) : 8144 -8154 . DOI: 10.12418/CJAN2025.664

Abstract

Short chain fatty acids (SCFA), medium chain fatty acids (MCFA) and polyunsaturated fatty acids (PUFA) are common natural nutrients, they show good efficacy in regulating the intestinal health of animals. In this paper, common functional fatty acids such as SCFA, MCFA and PUFA were reviewed, and the regulatory role of these kinds of common fatty acids in animal intestinal health was discussed from the aspects of intestinal cell and tissue morphology, immune function and microbiota; and so on, in order to provide references for these kinds of common fatty acids in applications of animal intestinal health and animal production.

随着经济的发展,消费者对肉类的需求呈不断上升的趋势。促生长类药物饲料添加剂的使用可加快畜禽生长发育,提高生产效率,但过度使用抗生素类饲料添加剂会造成病原菌的耐药性和动物产品的药物残留,严重危害了生态环境。随着全面禁抗,越来越多的替抗手段被投入研究,营养调控作为一种高效手段被广泛应用在畜禽生产中[1]。脂肪酸是一种由碳、氢、氧3种元素组成的营养素,并作为饲料添加剂应用于畜禽生产[2-3]
脂肪酸根据碳原子数量可分为短链脂肪酸(short chain fatty acid,SCFA)、中链脂肪酸(medium chain fatty acid,MCFA)和长链脂肪酸(long chain fatty acid,LCFA)。LCFA根据碳碳双键分为饱和脂肪酸和不饱和脂肪酸,不饱和脂肪酸又可分为单不饱和脂肪酸(monounsaturated fatty acid,MUFA)和多不饱和脂肪酸(polyunsaturated fatty acid,PUFA)。典型的多不饱和脂肪酸有n-3 PUFA、n-6 PUFA和n-9 PUFA,同时,根据动物体内能否自行合成可分为必需脂肪酸和非必需脂肪酸[4]。肠道作为动物机体主要消化吸收器官和重要免疫器官,维护肠道健康对动物机体健康至关重要。脂肪酸作为一种常见的营养素,能够通过调节肠道细胞和组织形态[5]、免疫功能[6]和微生态水平[7]来维护肠道健康。本文综述了几种常见脂肪酸(SCFA、MCFA、PUFA)在维护肠道健康中的作用机制及其在动物生产中的应用研究进展,以期为脂肪酸在调控动物体肠道健康和动物生产中的应用方面提供参考。

1 几种常见脂肪酸概述

1.1 SCFA

SCFA是碳原子数小于等于6个的脂肪酸,由肠道内微生物发酵不可消化的碳水化合物产生[4]。研究表明,SCFA可作为能量基底物质,亦可作为调节物质调节机体代谢,肠道中产生的SCFA主要有乙酸、丁酸、丙酸和戊酸,其中丁酸作为代表物质,是肠道细胞的主要能量来源[4,8]。Zhou等[9]将12头新生猪置于无菌隔离器中进行无菌饲养21 d,在第2个21 d期间,6头猪每天口服25 mL/kg无菌生理盐水作为无菌组,另6头猪每天口服25 mL/kg SCFA混合物(乙酸、丙酸和丁酸分别为45、15和11 mmol/L)作为SCFA组,结果表明,与无菌组相比,SCFA组脂肪沉积减轻,肝脏和背最长肌的葡萄糖调控改善,并且这一过程独立于肠道微生物群。T细胞亚群γδT细胞是T淋巴细胞的组成部分,γδT细胞对感染或炎症反应迅速,可被募集到损伤部位促进炎症反应[10]。刘槃等[11]研究发现,丙酸钠(sodium propionate,SP)、丁酸钠(sodium butyrate,SB)以及乙酸钠(sodium acetate,SA)、SP和SB组成的混合SCFA处理的γδT细胞白细胞介素-17A(interleukin-17A,IL-17A)含量与对照组相比均显著降低,且可抑制γδT细胞IL-17A、抑制因子激酶kappa B(inhibitor of kappa B kinase,IKK)的表达及核因子-κB(nuclear factor-κB,NF-κB)的磷酸化水平,结果表明,SCFA能抑制γδT细胞IL-17A和NF-κB信号通路的激活,从而减轻机体的炎症反应。邓曼琦等[12]研究发现,SCFA能与G蛋白偶联受体43(G protein-coupled receptor 43,GPR43)结合,抑制炎性细胞的活性,SCFA还可通过NF-κB和丝裂原活化蛋白激酶(mitogen-activated protein kinases,MAPK)信号转导,抑制炎症因子产生,SCFA能维持肠黏膜屏障的完整性,减少肠道内的内毒素泄露,有效减轻炎症反应。

1.2 MCFA

MCFA是碳原子数为6~12个的脂肪酸,通常以中链甘油三酯(medium chain triglycerides,MCT)的形式存在于各种饲料中。MCFA在动物营养和胃肠道功能中起着重要作用,主要的MCFA有己酸(hexanoic acid,C6)、辛酸(octanoic acid,C8)、癸酸(decanoic acid,C10)和月桂酸(lauric acid,C12)[4]。MCFA对肠道屏障的维护具有良好的效果,Sadurní等[13]研究发现,与对照组相比,饲粮中添加1 kg/t受MCFA钠盐保护的SB,可增加断奶仔猪回肠黏膜杯状细胞(goblet cell,GC)数量,从而增强肠道屏障功能,对维护肠道健康具有正向作用。月桂酸作为一种MCFA,是椰子油的主要脂肪酸[14]。Rolinec等[15]在研究中将19头大白猪分为2组(9头饲喂基础饲粮,10头饲喂含3%椰子油的基础饲粮),饲喂14 d,在试验开始和结束时,取2组中每头猪的直肠拭子,用16S rRNA高通量扩增子测序来分析直肠微生物组的变化,结果表明,饲喂含3%椰子油的基础饲粮可提高直肠乳杆菌属(Lactobacillus)、拟普雷沃菌属(Alloprevotella)、双歧杆菌目(Bifidobacteriales)和乳杆菌目(Lactobacillales)相对丰度,降低棒状杆菌属(Corynebacterium)、光岗菌属(Mitsuokella)、嗜冷杆菌属(Psychrobacter)和假单胞菌目(Pseudomonadales)相对丰度,微生物组的积极变化表明椰子油具有选择性抗菌作用。MCFA能够缓解动物机体炎症,触珠蛋白是一种炎症急性期时相反应蛋白,机体处于应激状态时,血液中触珠蛋白含量明显增多[16]。Szuba-Trznadel等[17]研究发现,饲粮中添加0.1%~0.3%的MCFA能使仔猪血清触珠蛋白含量降低2倍以上,表明MCFA能缓解仔猪断奶期的炎症。

1.3 PUFA

PUFA是具有2个或2个以上碳碳双键的直链脂肪酸,碳原子数为18~22个,其与动物健康和患病风险密切相关,与许多慢性疾病息息相关[18]。n-3 PUFA和n-6 PUFA是两大主要的PUFA,属于必需脂肪酸,不能由体内自主合成和转化,需要从外界获取。n-3 PUFA是指脂肪酸分子中第1个不饱和键出现在碳链甲基端第3位的脂肪酸,主要类型包括α-亚麻酸(α-linolenic acid,ALA)、二十碳五烯酸(eicosapentaenoic acid,EPA)和二十二碳六烯酸(docosahexaenoic,DHA)[4]。研究表明,饲粮或饮食中的n-6 PUFA∶n-3 PUFA可能影响动物体和人类机体的炎症水平和代谢,进而调节慢性疾病[19-20]。Kim等[21]在研究中选用4和24月龄C57BL/6J雄性小鼠,下丘脑组织检测显示,与年轻小鼠相比,老年小鼠下丘脑中的促炎细胞因子肿瘤坏死因子-α(tumor necrosis factor-α,TNF-α)、白细胞介素-1β(interleukin-1β,IL-1β)和环氧合酶-2(cyclooxygenase-2,COX-2)的mRNA相对表达水平升高;同时,下丘脑脂肪酸含量检测显示,与年轻小鼠相比,老年小鼠下丘脑中不饱和脂肪酸含量较低,表明组织中脂肪酸组成与机体组织炎症水平有关。Charpentier等[22]在研究中用脂肪酸饲粮饲喂75~100 g的年轻雄性大鼠,与对照组相比,n-3 PUFA∶n-6 PUFA∶n-9 PUFA为1∶1∶4的饲粮能显著下调结肠诱导型一氧化氮合成酶(inducible nitric oxide synthase,iNOS)和COX-2表达,减少白细胞介素-6(interleukin-6,IL-6)和白三烯B4(leukotriene B4,LTB4)的产生,有降低结肠TNF-α的产生的趋势;n-3 PUFA∶n-6 PUFA∶n-9 PUFA为1∶4∶24的饲粮能显著降低结肠IL-6的产生,结果表明,饲粮中的n-3 PUFA通过减弱炎症标志物影响结肠炎的发展。Lo Conte等[23]研究发现,给予免疫缺陷模型(non obese diabetes,NOD)大鼠富含n-3 PUFA的抗炎饲粮(anti-inflammatory diet,AID),与正常饲粮相比,富含n-3 PUFA的AID能降低NOD大鼠的肠道通透性,增强肠道紧密连接蛋白封闭蛋白-1(claudin-1,CLDN-1)的mRNA相对表达水平,降低肠道组织中炎症因子IL-1β、白细胞介素-23(interleukin-23,IL-23)和白细胞介素-17(interleukin-17,IL-17)的mRNA相对表达水平,增加了肠道微生物α多样性,提高了与黏液再生相关的肠道微生物嗜黏蛋白阿克曼菌(Akkermansia muciniphila)和双歧杆菌属(Bifidobacterium)相对丰度,降低了单形拟杆菌(Bacteroides uniformis)和链球菌属(Streptococcus)相对丰度。

2 SCFA、MCFA和PUFA对动物体肠道健康的影响及其作用机制

2.1 SCFA、MCFA和PUFA对肠道细胞和组织形态的调节作用

Toll样受体(Toll-like receptors,TLR)在机体免疫调节中起到关键作用,它能作为外源病原体的传感器,诱导机体产生免疫反应[24]。研究表明,TLR的激活能为肠道树突细胞(dendritic cell,DC)的成熟提供关键信号[25]。DC作为一种抗原呈递细胞,能够识别抗原并将信号传递给T细胞以有效激活T细胞[26]。脂肪酸作为一种信号分子能够调节TLR活性,n-3 PUFA能够通过抑制TLR活性来影响DC的成熟,从而降低T细胞的活性,进而调节机体免疫反应[27]。此外,有研究发现,暴露于LCFA和MCFA能维持DC的吞噬功能,而单独暴露于LCFA则破坏了DC的抗原呈递能力,表明脂肪酸能通过调节DC的功能进而调节肠道的免疫能力[28]。He等[29]研究发现,哺乳动物体内微生物产生的SCFA能诱导肠上皮GC分化、黏液产生和提高肠上皮细胞(intestinal epithelial cell,IEC)完整性,改善年轻小鼠肠上皮细胞连接完整性。Martínez-Vallespín等[30]通过体外研究发现,3种MCFA在猪小肠上皮细胞(porcine intestinal columnar epithelial cells,IPEC-J2)系中对细菌生长速率和基因表达均有不同程度的影响,对细菌攻毒的肠道细胞有潜在的修复和保护作用。Lu等[31]在研究中通过设计5种不同的n-6 PUFA∶n-3 PUFA处理的饲粮饲喂断奶仔猪,结果表明饲粮n-6 PUFA∶n-3 PUFA的增加有可能改变炎症压力下空肠的隐窝深度,对猪肠道形态影响至关重要。Wang等[32]研究发现,与基础饲粮相比,饲粮中添加2 000 mg/kg的功能性脂肪酸(主要组成为31.4%丁酸、2.77%辛酸和2.17%癸酸)降低了仔猪回肠隐窝深度。You等[33]研究表明,从母猪妊娠85 d开始到哺乳期结束,在母猪基础饲粮中添加SB和MCFA组合(1 g/kg包被SB和7.75 g/kg包被MCFA),SB和n-3 PUFA组合(1 g/kg包被SB和68.2 g/kg包被n-3 PUFA),MCFA和n-3 PUFA组合(7.75 g/kg包被MCFA和68.2 g/kg包被n-3 PUFA),SB、MCFA和n-3 PUFA组合(1 g/kg包被SB、7.75 g/kg包被MCFA和68.2 g/kg包被n-3 PUFA),结果表明,与对照组相比,饲喂4种不同的脂肪酸组合能使哺乳仔猪空肠黏膜CLDN-1和闭锁小带蛋白-1(zonula occludens-1,ZO-1)mRNA相对表达水平显著提高,有助于缓解哺乳仔猪腹泻,能增强肠道屏障功能;与对照组相比,饲喂4种不同的脂肪酸组合能使哺乳仔猪空肠绒毛高度/隐窝深度显著升高,对维护肠道健康具有积极作用。Upadhaya等[34]研究发现,在基础饲粮中添加包被SB(含400 g/kg SB和600 g/kg氢化棕榈油)饲喂断奶仔猪6周,分为3个不同剂量组(低剂量组:饲喂0.50 g/kg CSB至结束;中剂量组:饲喂1.50 g/kg CSB 3周后降至0.75 g/kg CSB至结束;高剂量组:饲喂3.00 g/kg CSB 3周后降至1.50 g/kg CSB至结束),结果表明,与对照组相比,3个不同剂量组的断奶仔猪十二指肠、空肠和回肠的绒毛长度显著增加,并对小肠微生物菌群产生积极影响。

2.2 SCFA、MCFA和PUFA对肠道免疫功能的调节作用

肠道的免疫水平与肠道内的免疫细胞有关,肠道内的免疫细胞主要包括先天淋巴样细胞、巨噬细胞、DC、B细胞和T细胞等;肠道免疫细胞位于肠道上皮组织、固有层和肠道淋巴组织中,当机体受到病原体侵袭时,肠道免疫细胞被有效激活以清除病原体,防止机体组织损伤[26,35]。富含饱和脂肪酸和丰富碳水化合物的饲粮在动物试验中被定义为高脂饲粮(high-fat diet,HFD),研究表明,HFD能通过直接影响免疫细胞亚群来改变肠道免疫反应,并通过影响肠道微生物群或肠上皮细胞间接影响肠道免疫细胞亚群[36]。Ferrara等[37]在研究中将72头断奶仔猪分为3组,对照组饲喂基础饲粮,SOA组在基础饲粮的基础上添加短链有机酸(0.41%富马酸+0.32%乳酸),SOA+MCFA组在基础饲粮的基础上添加短链有机酸和MCFA的混合物(0.15%辛酸和癸酸),饲喂28 d,结果表明,与对照组相比,SOA组断奶仔猪空肠上皮T细胞分化抗原2(cluster of differentiation 2,CD2)和T细胞分化抗原8(cluster of differentiation 8,CD8)数量显著增加,表明短链有机酸可以通过增加潜在效应细胞的组成数量来对抗传染病,从而对局部免疫产生有益的影响。炎症是机体的一种自我保护机制,适当的炎症对机体有益,过度的炎症会损伤机体[38]。Sundaram等[39]研究发现,在花生四烯酸(arachidonic acid,ARA)富集的细胞膜中,病原体、内毒素和某些非病原体应激因子能与宿主特异性受体结合,进而激活NF-κB信号通路,释放促炎物质,引发促炎反应,破坏紧密连接蛋白和上皮完整性,而n-3 PUFA能代替ARA改善促炎反应,并刺激抗炎因子的产生,进而修复肠道损伤。n-3 PUFA对炎症反应有抑制作用,但过量的n-3 PUFA可能会起到相反效果。Schwarzler等[40]研究发现,对2只小鼠模型进行了表型分析和机制解剖,其IEC特异性缺失X-box结合蛋1(X-box binding protein 1,XBP1)或谷胱甘肽过氧化酶4(glutathione peroxidase 4,GPx4)而表现出内质网(endoplasmic reticulum,ER)应激,对小鼠饲喂过量的PUFA能使特异性小鼠产生ER应激和肠炎。
Wang等[32]研究发现,与饲喂基础饲粮相比,饲粮中添加2 000 mg/kg的功能性脂肪酸(主要组成为31.4%丁酸、2.77%辛酸和2.17%癸酸)能降低仔猪空肠TNF-α、IL-1β、白细胞介素-8(interleukin-8,IL-8)和白细胞介素-10(interleukin-10,IL-10)含量,缓解仔猪肠道炎症;在饲喂第14天时,仔猪空肠过氧化氢酶(catalase,CAT)活性显著升高;在饲喂第28天时,仔猪空肠免疫球蛋白A(immunoglobulin A,IgA)和免疫球蛋白M(immunoglobulin M,IgM)含量显著升高。初乳中的免疫球蛋白是新生仔猪被动免疫的唯一来源,You等[33]研究发现,在母猪基础饲粮中添加SB+MCFA、MCFA+n-3 PUFA和SB+MCFA+n-3 PUFA 3种组合脂肪酸饲喂,增加了初乳中IgA和免疫球蛋白G(immunoglobulin G,IgG)的含量,表明了SB、MCFA和n-3 PUFA对免疫功能的积极调节作用;相较于对照组,3种脂肪酸组合饲喂能降低仔猪空肠黏膜炎症因子IL-1βTNF-αTLR4的mRNA相对表达水平,提高仔猪血浆谷胱甘肽过氧化物酶(glutathione peroxidase,GSH-Px)、总超氧化物歧化酶(total superoxide dismutase,T-SOD)、CAT活性和总抗氧化能力(total antioxidant capacity,T-AOC),对仔猪肠道炎症具有改善作用。Lo Conte等[23]在研究中通过对NOD小鼠饲喂AID,能改善NOD小鼠的免疫耐受机制,NOD小鼠的肠黏膜中叉头框蛋白P3+调节性T细胞(forkhead box P3+regulatory T cells,FoxP3+Treg)和10+1类调节性细胞(interleukin-10+type 1 regulatory T cells,IL-10+Tr1)分化增加,效应T细胞(effector T cells,Teff)分化减少,肠道、胰腺淋巴结和胰岛内淋巴细胞中效应辅助性T细胞17(T helper cell 17,Th17)和辅助性T细胞1(T helper cell 1,Th1)分化减少。Kuang等[41]在研究中通过与添加氧化锌的对照组相比,添加3 g/kg MCFA和有机酸混合物(甲酸钙、乳酸钙、柠檬酸和MCFA含量分别为340、160、70和130 g/kg)替代氧化锌进行饲喂,能显著降低血浆中TNF-α含量,显著提高血浆中IgG含量;显著下调空肠促炎细胞因子TNF-α的表达,对调节肠道炎症有积极作用。小泛素样酰化修饰(small ubiquitin-like modifier acylation,SUMOylation)是一种必需的泛素样修饰方式,参与多种肠道内炎症反应[42]。Ezzine等[43]研究表明,肠道微生物群产生的SCFA和BCFA以pH依赖的方式增加肠细胞中的蛋白质SUMOylation,BCFA能上调肠细胞的SUMOylation并抑制炎症反应,BCFA能抑制NF-κB信号通路,降低促炎细胞因子表达,促进肠上皮完整性。

2.3 SCFA、MCFA和PUFA对肠道微生物的调节作用

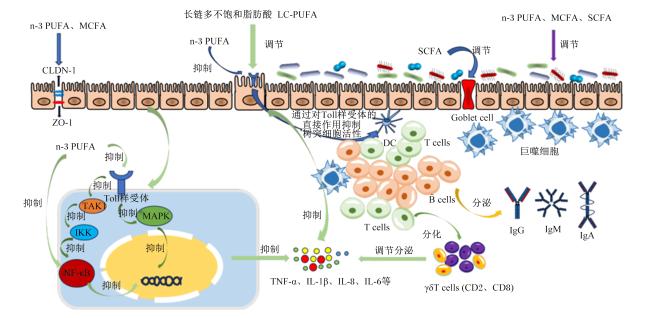
动物肠道内含有大量微生物,肠道内微生物种群的结构和多样性对维持动物肠道健康起着关键作用,肠道微生物对宿主的健康有着重要的影响[44]。肠道微生物对动物机体疾病和肠道疾病有着重要的调节作用,肠道微生物及其代谢物能调节肠道炎症和机体代谢[45-46]。厚壁菌门(Firmicute)、拟杆菌门(Bacteroidota)、变形菌门(Proteobacteria)和放线菌门(Actinobacteriota)在哺乳仔猪结肠内容物中占主导地位[47]。研究表明,n-3 PUFA能直接调节动物肠道微生物群的多样性和相对丰度,Firmicute和Bacteroidota是人体肠道内两大主要细菌门,Firmicute与Bacteroidota的比值升高,将导致肥胖等代谢性疾病,n-3 PUFA能直接改变其比值来调节肠道免疫[48]。Sebastia等[49]研究发现,肠道内不同的细菌属与脂肪酸谱之间存在显著相关性,直肠内容物中正丁酸与普雷沃氏菌属(Prevotella)呈显著正相关,与阿克曼氏菌属(Akkermansia)呈显著负相关,乙酸与PrevotellaAkkermansia呈显著负相关,表明了脂肪酸与肠道微生物之间的相互调节作用。Robertson等[50]研究表明,母体n-3 PUFA暴露减少导致变形菌纲(Epsilonproteobacteria)、拟杆菌属(Bacteroides)和Akkermansia相对丰度显著减少,而梭状芽孢杆菌属(Clostridia)相对丰度显著升高。在妊娠期或哺乳期,较低的母体n-6 PUFA∶n-3 PUFA显著降低了饲喂HFD后代的体重增加和代谢紊乱,这与肠道微生物群的持续重组介导有关,表明了n-3 PUFA在调节肠道菌群中的正向作用。Wang等[51]在研究中用3种不同n-6 PUFA∶n-3 PUFA饲粮(n-6 PUFA∶n-3 PUFA分别为8∶1、5∶1和3∶1)饲喂黑盖育肥猪,结果显示低n-6 PUFA∶n-3 PUFA饲粮能显著降低栖瘤胃解纤维素菌属(Cellulosilyticum)、BacteroidesAlloprevotella相对丰度,显著提高史雷克氏菌属(Slackia)和芽孢杆菌属(Sporobacter)相对丰度,对维护肠道健康具有积极作用。Lopez-Colom等[52]研究发现,在饲粮中添加从含有月桂酸的蒸馏椰子油中提取的MCFA能降低沙门氏菌属(Salmonella)攻击后断奶仔猪结肠Firmicute与Bacteroidota的比值,并富集纤维杆菌门(Fibrobacteres);在肠产毒性大肠杆菌(enterotoxigenic Escherichia coli,ETEC)F4+的攻毒下,MCFA混合物能使微生态结构发生变化,小杆菌属(Dialister)相对丰度升高,韦荣球菌科(Veillonellaceae)相对丰度有升高趋势,MCFA混合物在一定程度上能调节回肠的局部免疫,调节结肠微生物群,体现了MCFA混合物在减少肠道病原体和控制断奶前后肠道疾病方面的潜力。You等[33]研究发现,用SB与MCFA联合饲喂妊娠后期至哺乳期结束的母猪,可使仔猪结肠食糜中连环杆菌属(Catenbacterium)、粪球菌属(Coprococcus)、布雷德菌属(Bulleidia)、Prevotella和布劳特氏菌属(Blautia)相对丰度升高,Firmicute相对丰度降低;用MCFA与n-3 PUFA联合饲喂能使柯林斯氏菌属(Collinsella)、BlautiaBulleidia相对丰度升高,Firmicute相对丰度降低;用SB、MCFA和n-3 PUFA联合饲喂能使粪杆菌属(Faecalibacterium)和Bacteroidota相对丰度升高,Firmicute相对丰度降低;3种联合饲喂方案都能使结肠微生物群β多样性显著变化,促进仔猪肠道健康。脂肪酸对肠道损伤修复的作用机制见图1
图1 脂肪酸对肠道损伤修复的作用机制

n-3 PUFA:n-3多不饱和脂肪酸 n-3 polyunsaturated fatty acid;MCFA:中链脂肪酸 medium chain fatty acid;SCFA:短链脂肪酸 short chain fatty acid;CLDN-1:封闭蛋白-1 claudin-1;ZO-1:闭锁小带蛋白1 zonula occludens-1;TLR:Toll样受体 Toll-like receptors;TAK1:转化生长因子激酶1 transforming growth factor-β-activated kinase 1;IKK:抑制因子激酶kappa B inhibitor of kappa B kinase;NF-κB:核因子-κB nuclear factor-κB;MAPK:丝裂原活化蛋白激酶 mitogen-activated protein kinases;DC:肠道树突细胞 dendritic cell;GC:杯状细胞 goblet cell;TNF-α:肿瘤坏死因子-α tumor necrosis factor-α;IL-1β:白细胞介素-1β interleukin-1β;IL-8:白细胞介素-8 interleukin-8;IL-6:白细胞介素-6 interleukin-6;CD2:T细胞分化抗原2 cluster of differentiation 2;CD8:T细胞分化抗原8 cluster of differentiation 8;γδT:γδT细胞γδT cell;IgG:免疫球蛋白G immunoglobulin G;IgM:免疫球蛋白M immunoglobulin M;IgA:免疫球蛋白A immunoglobulin A;T cells:T淋巴细胞 T lymphocytes;B cells:B淋巴细胞 B lymphocytes。

Fig.1 Mechanisms of fatty acids on intestinal injury repair

3 SCFA、MCFA和PUFA在动物生产中的应用

脂肪酸作为饲料添加剂已经广泛应用于动物生产中[53-54]。利用藻类发酵产生脂肪酸是一种生产脂肪酸添加剂的新型手段[55]。Nayak等[56]研究发现,在饲料中添加富含长链多不饱和脂肪酸(long chain-polyunsaturated fatty acids,LC-PUFA)的微藻升高了斑马鱼与ARA代谢相关的COX-2、脂氧合酶-1(lipoxygenase-1,LOX-1)、IL-10、溶菌酶(lysozyme,LYZ)、肠道碱性磷酸酶(intestinal alkaline phosphatase,IAP)、补体3B(complement 3B,C3B)、CATGSH-Px等基因的相对表达水平;调节了斑马鱼的黏膜免疫功能,增加了肠道微生物多样性,促进了肠道健康,对肠道微生物稳态的维持具有重要作用。沈铭等[57]研究发现,饲粮中添加2%复合油脂(提高了MCFA、n-3 PUFA和部分饱和LCFA含量,降低了部分饱和LCFA和n-6 PUFA含量)等量替代2%的大豆油饲喂断奶仔猪,结果显示净能体系下复合油脂等量替代大豆油显著升高了猪肠道黏膜中GSH-Px活性,显著提高了CLDN-1和闭锁小带蛋白-2(zonula occludens-2,ZO-2)的蛋白相对表达水平,显著改变了粪便微生物门水平的β多样性,显著提高了Firmicutes相对丰度,显著降低了Bacteroidota相对丰度,表明复合油脂中的脂肪酸对维护肠道屏障功能、维持肠道健康具有积极作用。范国强等[58]研究发现,在对照组的基础上饲喂含0.5%的α-亚麻酸能促进育肥猪结肠瘤胃球菌科(Ruminococcaceae)、毛螺菌科(Lachnospiraceae)、Veillonellaceae、丁酸球菌科(Butyricicoccaceae)等SCFA产生菌的增殖,增加了Firmicutes的相对丰度,促进了肠道微生物多样性。雷昕茹等[59]研究发现,在基础饲粮中添加MCFA混合物增加了肉鸡血清中IgA、白细胞介素-4(interleukin-4,IL-4)含量,降低了IL-6、TNF-α、IL-1β、白细胞介素-18(interleukin-18,IL-18)含量,改善了GSH-Px活性和T-AOC,降低了丙二醛(malondialdehyde,MDA)含量,提高了肉鸡肠道绒毛高度和高绒毛高度/隐窝深度,降低了肉鸡盲肠内容物中Salmonella和ETEC的数量,提高了盲肠内容物中Lactobacillus的数量,改善了肠道健康。
燕磊等[60]研究表明,使用不同剂型丁酸添加剂对肉鸡生长性能和肠道健康均有促进作用,饲粮中添加丁酸可提高十二指肠中丁酸含量。张华等[61]在研究中选取840羽15周龄京粉1号蛋鸡,相较于饲喂基础饲粮,饲粮中添加1 000 mg/kg功能性脂肪酸复合物能显著提高20周龄蛋鸡血清GSH-Px活性,显著降低过氧化氢(H2O2)含量;显著降低28周龄蛋鸡血清CAT活性,显著降低血清MDA和H2O2含量,显著提高空肠GSH-Px活性,显著降低空肠MDA含量;显著提高20周龄蛋鸡血清IgG含量,显著提高24和28周龄蛋鸡血清IgM含量;显著提高28周龄蛋鸡空肠和回肠绒毛高度,显著降低隐窝深度,显著提高绒毛高度/隐窝深度,对蛋鸡的肠道健康和炎症调节均有积极作用。Li等[62]在研究中选取120头健康的断奶仔猪,随机分为5组,分别饲喂基础饲粮、低脂饲粮、低脂饲粮+SB、低脂饲粮+MCFA和低脂饲粮+n-3 PUFA,结果显示,与饲喂基础饲粮相比,饲喂低脂饲粮+SB、低脂饲粮+MCFA和低脂饲粮+n-3 PUFA降低了仔猪血浆中IL-8含量,提高了GSH-Px活性,降低了仔猪结肠黏膜TLR4 mRNA相对表达水平;饲喂低脂饲粮+SB和低脂饲粮+n-3 PUFA降低了仔猪结肠黏膜抑制因子激酶kappa B-α(inhibitor of kappa B kinase-α,IKK-α)mRNA相对表达水平;饲喂低脂饲粮+MCFA提高了仔猪结肠黏膜核因子红系2相关因子2(nuclear factor-erythroid 2 related factor 2,Nrf2)mRNA相对表达水平。上述结果表明,低脂饲粮中添加SB、MCFA或n-3 PUFA对仔猪肠道健康有重要作用。Lopez-Colom等[63]在饲粮中添加MCFA保护的SB能增加断奶仔猪回肠大肠杆菌和GC数量,增加Firmicute与Bacteroidota的比值,MCFA保护的SB对结肠内ETEC F4+具有抑制作用,MCFA保护的SB对肠上皮具有潜在营养作用,能增强肠道屏障。Duan等[64]研究发现,用不同的n-6 PUFA∶n-3 PUFA饲粮饲喂生长育肥猪,结果表明,饲粮中n-6 PUFA∶n-3 PUFA的最佳比例为1∶1和5∶1,可显著抑制炎症因子IL-1βTNF-αIL-6的mRNA表达,对脂质代谢和炎症系统均具有有益影响。

4 小结

在全面禁抗的时代,营养调控和绿色添加剂调控手段已经成为改善动物机体性状和调节动物机体健康的重要手段。SCFA、MCFA和PUFA作为天然的基础营养素,具有绿色、安全、无副作用和效果显著等优点,具有良好的应用前景。但SCFA、MCFA和PUFA的最佳使用剂量和具体使用剂量尚不明确,且其适口性是值得注意的问题。在SCFA、MCFA和PUFA生产工艺中,考虑到体内的代谢,如何使其在体内行使最佳的代谢途径也是其生产中需要面临的问题。总之,SCFA、MCFA和PUFA具有良好的饲用前景,需要进一步开发其潜在的营养价值。
[1]
郭祥. 畜牧业生产的营养管理策略[J]. 畜牧兽医科技信息, 2023(12):57-59.

GUO X. Nutritional management strategies for livestock production[J]. Chinese Journal of Animal Husbandry and Veterinary Medicine, 2023(12):57-59. (in Chinese)

[2]
周鹏, 宋晨, 池仕红, 等. 复合脂肪酸对母猪繁殖性能、仔猪抗氧化性能和免疫性能的影响[J]. 饲料研究, 2024, 47(4):29-33.

ZHOU P, SONG C, CHI S H, et al. Effects of compound fatty acids on reproductive performance of sows,antioxidant performance and immune performance of piglets[J]. Feed Research, 2024, 47(4):29-33. (in Chinese)

[3]
霍亚飞, 杨占江, 韩秋月. 日粮中添加油脂对蛋鸡的影响[J]. 中国动物保健, 2024, 26(4):89-90.

HUO Y F, YANG Z J, HAN Q Y. The effect of adding oil and fat to the diet on laying hens[J]. China Animal Health, 2024, 26(4):89-90. (in Chinese)

[4]
TVRZICKA E, KREMMYDA L S, STANKOVA B, et al. Fatty acids as biocompounds:their role in human metabolism,health and disease—a review.Part 1:classification,dietary sources and biological functions[J]. Biomedical Papers of the Medical Faculty of the University Palacky,Olomouc,Czechoslovakia, 2011, 155(2):117-130.

[5]
LIU P Y, WANG Y B, YANG G, et al. The role of short-chain fatty acids in intestinal barrier function,inflammation,oxidative stress,and colonic carcinogenesis[J]. Pharmacological Research, 2021, 165:105420.

DOI

[6]
YAO Y, CAI X Y, FEI W D, et al. The role of short-chain fatty acids in immunity,inflammation and metabolism[J]. Critical Reviews in Food Science and Nutrition, 2022, 62(1):1-12.

DOI

[7]
ZENG H W, UMAR S, RUST B, et al. Secondary bile acids and short chain fatty acids in the colon:a focus on colonic microbiome,cell proliferation,inflammation,and cancer[J]. International Journal of Molecular Sciences, 2019, 20(5):1214.

DOI

[8]
ZHANG L, LIU C D, JIANG Q Y, et al. Butyrate in energy metabolism:there is still more to learn[J]. Trends in Endocrinology and Metabolism, 2021, 32(3):159-169.

DOI

[9]
ZHOU H, YU B, SUN J, et al. Short-chain fatty acids can improve lipid and glucose metabolism independently of the pig gut microbiota[J]. Journal of Animal Science and Biotechnology, 2021, 12(1):61.

DOI PMID

[10]
闫新宇, 韩金帅, 王俊阁. γδT细胞在气道过敏性疾病中的作用[J]. 中国临床医生杂志, 2024, 52(1):29-31.

YAN X Y, HAN J S, WANG J G. The role of γδT cells in airway allergic diseases[J]. Chinese Journal for Clinicians, 2024, 52(1):29-31. (in Chinese)

[11]
刘槃, 席德双, 黄瑞, 等. 短链脂肪酸通过抑制白细胞介素17A和NF-κB信号通路减轻γδT细胞介导的炎症反应[J]. 实用医学杂志, 2024, 40(8):1088-1094.

LIU P, XI D S, HUANG R, et al. Short-chain fatty acids alleviate γδT cell-mediated inflammatory response via inhibiting IL-17A and NF-κB signaling pathway[J]. The Journal of Practical Medicine, 2024, 40(8):1088-1094. (in Chinese)

[12]
邓曼琦, 顾兵, 吴思颖, 等. 短链脂肪酸促进痛风炎症反应消散作用的研究进展[J]. 江西科学, 2024, 42(2):257-263.

DENG M Q, GU B, WU S Y, et al. Research progress of short-chain fatty acids promoting the dissipation of gout inflammatory response[J]. Jiangxi Science, 2024, 42(2):257-263. (in Chinese)

[13]
SADURNÍ M, BARROETA A C, SOL C, et al. Effects of dietary crude protein level and sodium butyrate protected by medium-chain fatty acid salts on performance and gut health in weaned piglets[J]. Journal of Animal Science, 2023,101:skad090.

[14]
SCHWINGSHACKL L, SCHLESINGER S. Coconut oil and cardiovascular disease risk[J]. Current Atherosclerosis Reports, 2023, 25(5):231-236.

DOI PMID

[15]
ROLINEC M, MEDO J, GÁBOR M, et al. The effect of coconut oil addition to feed of pigs on rectal microbial diversity and bacterial abundance[J]. Animals, 2020, 10(10):1764.

DOI

[16]
QUAYE I K. Haptoglobin,inflammation and disease[J]. Transactions of the Royal Society of Tropical Medicine and Hygiene, 2008, 102(8):735-742.

DOI

[17]
SZUBA-TRZNADEL A, HIKAWCZUK T M, FUCHS B, et al. Effect of the supplementtaion of medium-chain fatty acids to mixtures containing zinc oxide nanoparticles on the growth performance and selected biochemical parameters of blood serum in pigs[J]. Journal of Elementology, 2019, 24(4):1203-1214.

[18]
娄毛闪, 于海宁, 沈生荣. 膳食亚油酸与肠道菌群和慢性代谢性疾病的关系[J]. 现代医药卫生, 2023, 39(21):3611-3614,3619.

LOU M S, YU H N, SHEN S R. Association of dietary linoleic acid with gut microbiome and chronic metabolic diseases[J]. Journal of Modern Medicine and Health, 2023, 39(21):3611-3614,3619. (in Chinese)

[19]
王琼. 不饱和脂肪酸对肥胖患者脂代谢和脂肪酸分布的影响[D]. 博士学位论文. 无锡: 江南大学, 2023.

WANG Q. Effects of unsaturated fatty acids on lipid metabolism and fatty acid distribution in obese patients[D]. Ph.D.Thesis. Wuxi: Jiangnan University, 2023. (in Chinese)

[20]
苏杭. 亚油酸和α-亚麻酸的摄入比例对体内炎症因子及高度不饱和脂肪酸合成通路的影响[D]. 博士学位论文. 无锡: 江南大学, 2018.

SU H. Effect of linoleic acid/alpha-linolenic acid ratio on inflammatory markers and HUFA biosynthesis pathway[D]. Ph.D.Thesis. Wuxi: Jiangnan University, 2018. (in Chinese)

[21]
KIM Y J, TU T H, YANG S, et al. Characterization of fatty acid composition underlying hypothalamic inflammation in aged mice[J]. Molecules, 2020, 25(14):3170.

DOI

[22]
CHARPENTIER C, CHAN R, SALAMEH E, et al. Dietary n-3 PUFA may attenuate experimental colitis[J]. Mediators of Inflammation, 2018, 2018:8430614.

[23]
LO CONTE M, ANTONINI CENCICCHIO M, ULASZEWSKA M, et al. A diet enriched in omega-3 PUFA and inulin prevents type 1 diabetes by restoring gut barrier integrity and immune homeostasis in NOD mice[J]. Frontiers in Immunology, 2023, 13:1089987.

DOI

[24]
ALURI J, COOPER M A, SCHUETTPELZ L G. Toll-like receptor signaling in the establishment and function of the immune system[J]. Cells (Basel,Switzerland), 2021, 10(6):1374.

[25]
KAMDAR K, NGUYEN V, DEPAOLO R W. Toll-like receptor signaling and regulation of intestinal immunity[J]. Virulence, 2013, 4(3):207-212.

DOI PMID

[26]
RIVERA C A, LENNON DUMENIL A M. Gut immune cells and intestinal niche imprinting[J]. Seminars in Cell & Developmental Biology, 2023,150/151:50-57.

[27]
WEATHERILL A R, LEE J Y, ZHAO L, et al. Saturated and polyunsaturated fatty acids reciprocally modulate dendritic cell functions mediated through TLR4[J]. The Journal of Immunology, 2005, 174(9):5390-5397.

DOI

[28]
TSUZUKI Y, MIYAZAKI J, MATSUZAKI K, et al. Differential modulation in the functions of intestinal dendritic cells by long-and medium-chain fatty acids[J]. Journal of Gastroenterology, 2006, 41(3):209-216.

DOI

[29]
HE Z Y, DONG H. The roles of short-chain fatty acids derived from colonic bacteria fermentation of non-digestible carbohydrates and exogenous forms in ameliorating intestinal mucosal immunity of young ruminants[J]. Frontiers in Immunology, 2023, 14:1291846.

DOI

[30]
MARTÍNEZ-VALLESPÍN B, VAHJEN W, ZENTEK J. Effects of medium-chain fatty acids on the structure and immune response of IPEC-J2 cells[J]. Cytotechnology, 2016, 68(5):1925-1936.

DOI

[31]
LU N, MEYER T A, BRUCKNER G, et al. Effects of dietary n-6:n-3 fatty acid ratio on growth performance,plasma fatty acid profile,intestinal morphology,and immune function of pigs[J]. Livestock Science, 2020, 238:104042.

DOI

[32]
WANG H K, WANG Y N, ZHANG Y, et al. Effects of a functional fatty acid blend on growth performance,intestinal morphology,and serum profiles in weaned piglets[J]. Animal Bioscience, 2023, 36(5):761-767.

DOI

[33]
YOU C Y, XU Q Q, CHEN J C, et al. Effects of different combinations of sodium butyrate,medium-chain fatty acids and omega-3 polyunsaturated fatty acids on the reproductive performance of sows and biochemical parameters,oxidative status and intestinal health of their offspring[J]. Animals:an Open Access Journal from MDPI, 2023, 13(6):1093.

[34]
UPADHAYA S D, JIAO Y, KIM Y M, et al. Coated sodium butyrate supplementation to a reduced nutrient diet enhanced the performance and positively impacted villus height and faecal and digesta bacterial composition in weaner pigs[J]. Animal Feed Science and Technology, 2020, 265:114534.

DOI

[35]
WANG Q L, LU Q J, JIA S J, et al. Gut immune microenvironment and autoimmunity[J]. International Immunopharmacology, 2023, 124(Pt A):110842.

[36]
QIU J X, MA Y H, QIU J. Regulation of intestinal immunity by dietary fatty acids[J]. Mucosal Immunology, 2022, 15(5):846-856.

DOI PMID

[37]
FERRARA F, TEDIN L, PIEPER R, et al. Influence of medium-chain fatty acids and short-chain organic acids on jejunal morphology and intra-epithelial immune cells in weaned piglets[J]. Journal of Animal Physiology and Animal Nutrition (Berlin), 2017, 101(3):531-540.

DOI

[38]
GU Z N, SHAN K, CHEN H Q, et al. n-3 polyunsaturated fatty acids and their role in cancer chemoprevention[J]. Current Pharmacology Reports, 2015, 1(5):283-294.

DOI PMID

[39]
SUNDARAM T S, GIROMINI C, REBUCCI R, et al. Role of omega-3 polyunsaturated fatty acids,citrus pectin,and milk-derived exosomes on intestinal barrier integrity and immunity in animals[J]. Journal of Animal Science and Biotechnology, 2022, 13(1):40.

DOI

[40]
SCHWARZLER J, MAYR L, VILA A V, et al. PUFA-induced metabolic enteritis as a fuel for Crohn’s disease[J]. Gastroenterology, 2022, 162(6):1690-1704.

DOI

[41]
KUANG Y, WANG Y, ZHANG Y, et al. Effects of dietary combinations of organic acids and medium chain fatty acids as a replacement of zinc oxide on growth,digestibility and immunity of weaned pigs[J]. Animal Feed Science and Technology, 2015, 208:145-157.

DOI

[42]
KARHAUSEN J, ULLOA L, YANG W. SUMOylation connects cell stress responses and inflammatory control:lessons from the gut as a model organ[J]. Frontiers in Immunology, 2021, 12:646633.

DOI

[43]
EZZINE C, LOISON L, MONTBRION N, et al. Fatty acids produced by the gut microbiota dampen host inflammatory responses by modulating intestinal sumoylation[J]. Gut Microbes, 2022, 14(1):2108280.

DOI

[44]
MARCHESI J R, ADAMS D H, FAVA F, et al. The gut microbiota and host health:a new clinical frontier[J]. Gut, 2015, 65(2):330-339.

DOI

[45]
AGUS A, CLÉMENT K, SOKOL H. Gut microbiota-derived metabolites as central regulators in metabolic disorders[J]. Gut, 2021, 70(6):1174-1182.

DOI PMID

[46]
LLOYD-PRICE J, ARZE C, ANANTHAKRISHNAN A N, et al. Multi-omics of the gut microbial ecosystem in inflammatory bowel diseases[J]. Nature, 2019, 569(7758):655-662.

DOI

[47]
DONG B, LIN X Q, JING X H, et al. A bacterial genome and culture collection of gut microbial in weanling piglet[J]. Microbiology Spectrum, 2022, 10(1):e02417-21.

[48]
FU Y W, WANG Y D, GAO H, et al. Associations among dietary omega-3 polyunsaturated fatty acids,the gut microbiota,and intestinal immunity[J]. Mediators of Inflammation, 2021, 2021:8879227.

DOI

[49]
SEBASTIA C, FOLCH J M, BALLESTER M, et al. Interrelation between gut microbiota,SCFA,and fatty acid composition in pigs[J]. mSystems, 2024, 9(1):e0104923.

DOI

[50]
ROBERTSON R C, KALIANNAN K, STRAIN C R, et al. Maternal omega-3 fatty acids regulate offspring obesity through persistent modulation of gut microbiota[J]. Microbiome, 2018, 6(1):95.

DOI PMID

[51]
WANG L Y, NONG Q Y, ZHOU Y B, et al. Changes in serum fatty acid composition and metabolome-microbiome responses of Heigai pigs induced by dietary n-6/n-3 polyunsaturated fatty acid ratio[J]. Frontiers in Microbiology, 2022, 13:917558.

DOI

[52]
LOPEZ-COLOM P, CASTILLEJOS L, RODRÍGUEZ-SORRENTO A, et al. Efficacy of medium-chain fatty acid salts distilled from coconut oil against two enteric pathogen challenges in weanling piglets[J]. Journal of Animal Science and Biotechnology, 2019, 10:89.

DOI

[53]
王海波, 占今舜, 霍俊宏, 等. 短链脂肪酸的生理功能及其在动物生产中的应用研究进展[J]. 中国畜牧杂志, 2023, 59(11):30-36.

WANG H B, ZHAN J S, HUO J H, et al. Research progress on physiological functions of short-chain fatty acids and its applications in animal production[J]. Chinese Journal of Animal Science, 2023, 59(11):30-36. (in Chinese)

[54]
周英焕, 刘小平, 高玉云, 等. 多不饱和脂肪酸的生物学功能及其在畜禽生产中的应用研究进展[J]. 中国畜牧杂志, 2024, 60(6):21-28.

ZHOU Y H, LIU X P, GAO Y Y, et al. Research progress on the biological functions and application of polyunsaturated fatty acids in livestock and poultry production[J]. Chinese Journal of Animal Science, 2024, 60(6):21-28. (in Chinese)

[55]
宫嘉泰, 胡睿智, 杨茜梓, 等. 裂殖壶藻的生理功能及其在畜牧生产中的应用[J]. 动物营养学报, 2022, 34(3):1476-1485.

DOI

GONG J T, HU R Z, YANG Q Z, et al. Biological function and application of Schizochytrium in livestock production[J]. Chinese Journal of Animal Nutrition, 2022, 34(3):1476-1485. (in Chinese)

[56]
NAYAK S, AL ASHHAB A, ZILBERG D, et al. Dietary supplementation with omega-6 LC-PUFA-rich microalgae regulates mucosal immune response and promotes microbial diversity in the zebrafish gut[J]. Biology(Basel), 2020, 9(6):119.

[57]
沈铭, 闫恩法, 何琳娟, 等. 饲粮中添加复合油脂等量替代大豆油对保育猪生长性能和肠道健康的影响[J]. 动物营养学报, 2024, 36(4):2218-2233.

DOI

SHEN M, YAN E F, HE L J, et al. Effects of replacement of equivalent amounts of soybean oil with compound oil in diets on growth performance and intestinal health of nursery pigs[J]. Chinese Journal of Animal Nutrition, 2024, 36(4):2218-2233. (in Chinese)

DOI

[58]
范国强, 张海, 栗艳飞, 等. 日粮添加α-亚麻酸对育肥猪肌肉脂肪酸组成与肠道菌群的影响[J]. 南京农业大学学报, 2024, 47(5):907-915.

FAN G Q, ZHANG H, LI Y F, et al. Effects of dietary α-linolenic acid supplementation on muscle fatty acid composition and intestinal flora of fattening pigs[J]. Journal of Nanjing Agricultural University, 2024, 47(5):907-915. (in Chinese)

[59]
雷昕茹, 孙耀威, 汪成飞, 等. 中链脂肪酸、植物精油和益生菌对肉鸡生长、免疫、抗氧化和肠道菌群及肌肉品质的影响[J]. 中国畜牧杂志, 2024, 60(2):391-396.

LEI X R, SUN Y W, WANG C F, et al. The effects of medium chain fatty acids,plant essential oils,and probiotics on the growth,immunity,antioxidant capacity,gut microbiota,and muscle quality of broiler chickens[J]. Chinese Journal of Animal Science, 2024, 60(2):391-396. (in Chinese)

[60]
燕磊, 安沙, 高佳, 等. 饲粮中添加不同剂型丁酸对肉鸡生长性能、肠道健康、脚垫和步态评分的影响[J]. 动物营养学报, 2023, 35(11):7002-7013.

DOI

YAN L, AN S, GAO J, et al. Effects of different butyric acid dosage forms in diets on growth performance,intestinal health,footrest and gait scores of broilers[J]. Chinese Journal of Animal Nutrition, 2023, 35(11):7002-7013. (in Chinese)

DOI

[61]
张华, 张双双, 王济华, 等. 脂肪酸复合物与绿原酸对蛋鸡生产性能与生理生化的影响[J]. 贵州农业科学, 2023, 51(10):73-84.

ZHANG H, ZHANG S S, WANG J H, et al. Effects of fatty acid complexes and chlorogenic acid on productive performance,physiology and biochemistry of laying hens[J]. Guizhou Agricultural Sciences, 2023, 51(10):73-84. (in Chinese)

[62]
LI W X, LAN T Y, DING Q, et al. Effect of low protein diets supplemented with sodium butyrate,medium-chain fatty acids,or n-3 polyunsaturated fatty acids on the growth performance,immune function,and microbiome of weaned piglets[J]. International Journal of Molecular Sciences, 2023, 24(24):17592.

DOI

[63]
LOPEZ-COLOM P, CASTILLEJOS L, RODRÍGUEZ-SORRENTO A, et al. Impact of in-feed sodium butyrate or sodium heptanoate protected with medium-chain fatty acids on gut health in weaned piglets challenged with Escherichia coli F4[J]. Archives of Animal Nutrition, 2020, 74(4):271-295.

DOI

[64]
DUAN Y H, LI F N, LI L L, et al. n-6∶n-3 PUFA ratio is involved in regulating lipid metabolism and inflammation in pigs[J]. British Journal of Nutrition, 2014, 111(3):445-451.

DOI

文章导航

/