综述

低聚糖作用于肠道的相关信号通路分析及其在断奶仔猪中的应用

  • 郑茗卉 , 1 ,
  • 张董燕 2 ,
  • 刘明 , 1, *
展开
  • 1 北京农学院动物科学技术学院,北京 102206
  • 2 北京市农林科学院畜牧兽医研究所,北京 100097
* 刘 明,教授,博士生导师,E-mail:

郑茗卉(2003—),女,辽宁鞍山人,硕士研究生,研究方向为猪营养与免疫。E-mail:

Office editor: 武海龙

收稿日期: 2025-06-20

  网络出版日期: 2026-02-12

基金资助

北京农学院人才强教工程(5066516008-6)

国家自然科学基金(32402781)

Analysis of Related Signaling Pathways of Oligosaccharides Acting on Intestinal Tract and Their Application in Weaned Piglets

  • ZHENG Minghui , 1 ,
  • ZHANG Dongyan 2 ,
  • LIU Ming , 1, *
Expand
  • 1 Animal Science and Technology College, Beijing University of Agriculture, Beijing 102206, China
  • 2 Institute of Animal Husbandry and Veterinary Medicine, Beijing Academy of Agriculture and Forestry Sciences, Beijing 100097, China
* professor, E-mail:

Received date: 2025-06-20

  Online published: 2026-02-12

摘要

动物机体健康面临着致病菌增多、热应激等问题,这些因素易导致动物肠道损伤、免疫抑制及代谢性疾病发生。低聚糖是一种由单糖通过糖苷键连接而成的低度聚合糖,作为一种功能性饲料添加剂,可作为益生元供肠道有益菌利用。低聚糖能够被肠道微生物代谢以及影响微生物群的代谢功能,在改善肠道屏障功能、肠道菌群平衡、肠道信号通路调控及免疫应答等方面发挥重要作用。本文从低聚糖常见种类和结构特点、低聚糖对动物肠道健康的调控作用进行了综述,进一步从抗氧化、宿主免疫和炎症通路方面阐述了低聚糖可能参与的信号通路和作用机制,并对其在断奶仔猪饲粮中的应用进行了总结分析,为低聚糖在畜牧养殖生产中的科学应用提供参考。

本文引用格式

郑茗卉 , 张董燕 , 刘明 . 低聚糖作用于肠道的相关信号通路分析及其在断奶仔猪中的应用[J]. 动物营养学报, 2026 , 38(2) : 823 -934 . DOI: 10.12418/CJAN2026.064

Abstract

Animal health is confronted with various problems, such as the increase in pathogenic bacteria and heat stress. These factors can easily lead to intestinal damage, immunosuppression and the occurrence of metabolic diseases in animals. Oligosaccharides are low-grade polymeric sugars formed by monosaccharides linked by glycosidic bonds, as a functional feed additive, can serve as prebiotics for the utilization of beneficial intestinal bacteria. Oligosaccharides can be metabolized by intestinal microorganisms and affect the metabolic function of the microbiota, which play important roles in improving intestinal barrier function, regulating the balance of intestinal microbiota, and controlling intestinal signaling pathways and immune responses. In this paper, we review the common types and structural characteristics of oligosaccharides, summarizes their regulatory effects on the animal gut health, and further elaborates on the possible signaling pathways and mechanisms of action of oligosaccharides from the aspects of antioxidant, host immunity and inflammatory pathways, in addition, we also review their application in the die of weaned piglets, to provide a reference is for the scientific application of oligosaccharides in animal production.

动物肠道是营养物质消化吸收的重要场所,能够维护机体健康和稳态。肠道内通过一系列复杂的内源和外源抗氧化机制,维持着肠道的氧化还原平衡,防止因氧化应激过度而导致细胞损伤[1]。肠道内存在着大量的免疫细胞,这些免疫细胞能够精准识别侵入肠道的病原体,并迅速启动免疫反应,有效抵御外界病菌的侵袭[2]。在炎症调控领域,肠道能够敏锐感知炎症信号,通过调节炎症相关因子的表达,控制炎症反应的程度和范围,避免炎症过度扩散对机体造成更大的伤害[3]。低聚糖作为一种功能性乳品添加剂,在肠道内可以被双歧杆菌等有益菌选择性利用[4],增加肠道内有益菌的数量,减少潜在致病菌的数量。低聚糖通过调控肠道菌群[5]和炎症因子表达,改善肠道免疫,进而促进动物生长[6-7]。低聚糖具有独特的生理活性,在改善动物肠道健康方面展现出巨大潜力。基于此,本文通过分析低聚糖常见种类和结构特点,阐述其对动物肠道调控的生物学功能,进一步分析了低聚糖参与的机体信号通路及作用机制,最后对低聚糖在断奶仔猪饲粮中的应用进行了总结,以期为推动低聚糖在畜牧业中的高效合理应用提供参考。

1 低聚糖种类及其对肠道的调控作用

1.1 低聚糖种类与结构特点

甘露寡糖(mannan oligosaccharides,MOS)通常是多个甘露糖残基线性连接而成的低聚糖(3~10个甘露糖残基),根据寡糖分子母链上糖苷键的类型不同可分为2类:α-MOS和β-MOS。α-MOS是由酵母细胞壁中的α-1,6-甘露聚糖水解,形成不同聚合度的低聚糖混合物;而β-MOS是由植物中的β-1,4-甘露聚糖水解,形成不同聚合度的低聚糖混合物[8]。褐藻寡糖(alginate oligosaccharides,AOS)广泛存在于海藻细胞壁中,是一种阴离子聚合物,由β-D-甘露糖醛酸(M)和α-L-古洛糖醛酸(G)通过1~4糖苷键连接而成的高分子化合物,主要通过酶解法获得[9]。AOS分为聚甘露糖醛酸(PM)、聚古罗糖醛酸(PG)和杂合褐藻寡糖(PMG)3种类型。低聚果糖(fructo oligosaccharides,FOS)由蔗糖分子以β-1,2糖苷键与1~3个果糖分子连接形成,是一种聚合度为2~9的功能性低聚糖,可分为蔗-果型和果-果型,其甜度仅为蔗糖的30%~60%,具体取决于其化学结构和聚合度[10-11]。低聚壳聚糖(chitosan oligosaccharides,COS)是由壳聚糖经过生物酶降解技术得到的聚合度在2~20的低聚糖产品[12]。COS分子链短,具有较高的溶解度,且容易被动物消化道吸收,是迄今为止发现自然界中唯一带正电荷的阳离子碱性低聚糖[13]

1.2 调节肠道物理屏障

肠道物理屏障是机体抵御外界病原体、毒素及抗原物质的第1道防线,主要由肠道上皮细胞以及黏液层组成[14],能够阻止大分子物质(如细菌、毒素)经细胞间隙穿透单层柱状上皮细胞屏障,且通过紧密连接、黏着连接和桥粒等结构形成连续屏障[15-16]。紧密连接中的闭锁蛋白、闭合蛋白等多种蛋白质参与形成选择性屏障,其通透性决定着肠上皮细胞的屏障功能。结肠黏液层是由杯状细胞分泌的黏蛋白构成,分为内层(致密,抗菌)和外层(松散,允许共生菌定植),具有润滑肠道、隔离微生物与上皮细胞的作用[17]。研究表明,低聚木糖(xylo-oligosaccharides,XOS)能够增加肉鸡回肠绒毛高度/隐窝深比和回肠中的杯状细胞数量[18]。MOS能够促进断奶仔猪十二指肠绒毛高度增加[19],对肠道形态产生有益影响。COS可以直接增强肠道屏障功能,减少炎症水肿,促进杯状细胞分泌黏蛋白,增加紧密连接蛋白的表达,恢复细胞间连接的完整性和密封性,促进肠道菌群的丰富性和多样性[20]

1.3 调控肠道微生物及代谢

肠道微生物包括细菌、古菌、真菌、原生动物和病毒,与宿主共同进化影响着肠道的生理功能。研究表明,低聚糖可以通过改善肠道微生物群,增加有益微生物来缓解黏膜炎,其在肠道内被微生物群分解后产生多种代谢产物,如短链脂肪酸(short-chain fatty acids,SCFAs)等发酵产物;还能影响肠道微生物群对胆汁酸进行代谢,这些代谢产物均能影响肠道上皮细胞的功能和肠道健康[21]。SCFAs是肠道微生物发酵产生的主要代谢产物,乙酸能调节肠道激素的分泌,影响食欲和能量摄入,参与体重和能量平衡的调节[22]。丙酸和丁酸通过激活免疫细胞上的G蛋白偶联受体,如G蛋白偶联受体43(G protein-coupled receptor 43,GPR43),调节免疫细胞的活性和功能,减轻肠道炎症,SCFAs可以调节肠道内的免疫应答,维持肠道免疫稳态[23]。胆汁酸能参与肠道脂肪的消化和吸收,抑制有害菌的生长,维护肠道健康,还可以参与脂肪代谢过程,通过激活法尼醇X受体,调节脂肪和胆固醇的代谢,促进脂肪的消化和吸收,影响能量平衡[24-25]。胆汁酸还可参与肠道免疫调节过程,能够影响免疫细胞的活性和分化,通过激活核因子-κB(nuclear factor-κB,NF-κB)信号通路,调节肠道内的炎症反应。

2 低聚糖调控动物肠道功能的相关信号通路

信号通路是一系列酶促反应构成的传导路径,可将细胞外的分子信号(即配体)经细胞膜传递至细胞内,并产生相应效应[26],配体涵盖激素、生长因子、细胞因子、神经递质及部分小分子化合物等[27]表1总结了低聚糖参与的信号通路及其对动物肠道健康的作用机制。
表1 低聚糖参与的信号通路及其对动物肠道健康的作用机制

Table 1 Signaling pathways involved in oligosaccharides and their mechanisms of action on animal intestinal health

低聚糖种类
Oligosaccharide types
作用机理及功能
Mechanism of action and function
参考文献
References
甘露寡糖MOS 调节Nrf2信号通路,减轻草鱼嗜水气单胞菌感染后头肾和脾脏的氧化损伤 [28]

褐藻寡糖AOS
激活Nrf2信号通路,改善D-半乳糖诱导的小鼠肾脏衰老 [29]
阻断FGF1介导的TLR4/NF-κB p65信号通路,减轻衰老相关肠黏膜屏障功能障碍 [30]
低聚果糖FOS 激活Nrf2信号传导,减少断奶仔猪腹泻,同时改善肠道抗氧化酶
活性和紧密连接蛋白表达
[31]


低聚壳聚糖COS
调节T84细胞中PI3K/AKT和ERK信号通路的相互作用,
促进连接屏障的完整性
[32]
调节线粒体凋亡和MAPK信号通路,减轻LPS引起的肠道炎症 [6]
调节HIF-1α信号通路,减轻H2O2刺激的颗粒细胞损伤 [33]
激活Nrf2/ARE信号通路,保护H2O2介导的氧化损伤和细胞凋亡 [34]

Nrf2:核因子E2相关因子2 nuclear factor erythroid 2-related factor 2;FGF1:成纤维细胞生长因子1 fibroblast growth factor 1;NF-κB p65:核因子-κB p65亚基 nuclear factor-κB p65 subunit;PI3K:磷脂酰肌醇3-激酶 phosphatidylinositol 3-kinase;AKT:蛋白激酶B protein kinase B;ERK:细胞外信号调节激酶 extracellular signal-regulated kinase;MAPK:丝裂原活化蛋白激酶 mitogen-activated protein kinase;HIF-1α:缺氧诱导因子-1α hypoxia-inducible factor-1 alpha;LPS:脂多糖 lipopolysaccharide;ARE:抗氧化反应元件 antioxidant response element;H2O2:过氧化氢 hydrogen peroxide。

2.1 调节肠道相关抗氧化通路

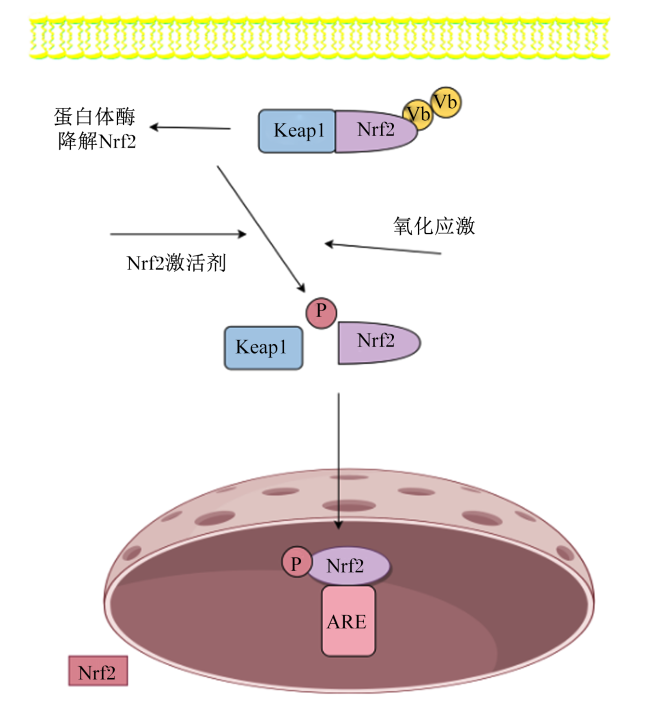
氧化应激是体内氧化与抗氧化作用失衡引起的,该过程会产生大量氧化中间产物,破坏细胞的结构,影响其生理功能。核因子E2相关因子2(nuclear factor erythroid 2-related factor 2,Nrf2)能结合到许多细胞保护基因启动子区域的抗氧化反应元件(antioxidant response element,ARE)上[35]。在正常情况下,Nrf2会被Kelch样环氧氯丙烷相关蛋白1(Kelch-like ECH-associated protein 1,Keap1)泛素化降解在细胞质中(图1);氧化应激条件下,亲电子代谢物抑制Keap1[36],它还参与β-珠蛋白基因转录激活[37],应激时激活Nrf2调控靶基因[38]。超氧化物歧化酶(superoxide dismutase,SOD)主要存在于细胞液和线粒体基质中,是防御生物体氧化损伤的一种金属酶[39],能保护生物细胞免受超氧自由基和由其形成的活性氧类的毒害[40]
图1 Nrf2信号通路(由Figdraw绘制)

Nrf2:核因子E2相关因子2 nuclear factor erythroid 2-related factor 2;Keap1:Kelch样环氧氯丙烷相关蛋白1 Kelch-like ECH-associated protein 1;ARE:抗氧化反应元件 antioxidant response element;Vb:维生素B vitamin B。

Fig.1 Nrf2 Signal pathways (drawn by Figdraw)

MOS的增强肠道抗氧化能力与Nrf2/Keap1信号通路的激活部分相关。研究发现,MOS能提升草鱼上皮细胞Nrf2的mRNA水平以及核内Nrf2蛋白水平,同时降低Keap1aKeap1b的mRNA水平,且除锰超氧化物歧化酶(manganese superoxide dismutase,MnSOD)外的抗氧化酶mRNA水平与肠道Nrf2蛋白水平呈正相关[41]。COS可有效缓解活动性炎症,恢复肠道上皮功能并减少肠道纤维化,可通过刺激Nrf2、增加内源性抗氧化剂的产生和减轻氧化应激来调节大鼠结肠组织的氧化还原稳态[42]

2.2 参与宿主免疫相关通路

低聚糖主要通过识别肠道免疫受体Toll样受体4(Toll-like receptor 4,TLR4)等,激活免疫信号通路Wnt/β-连环蛋白(β-catenin)信号通路等,促进免疫因子分泌,增强免疫功能。TLR4是低聚糖免疫调控的重要受体,能够识别多种分子模式,激活下游信号通路,引发免疫反应[43-44]。AOS可以与TLR4的接头蛋白结合,通过信号级联激活TLR4信号通路,如磷脂酰肌醇-3-激酶(phosphatidylinositol 3-kinase,PI3K)和蛋白激酶B(protein kinase B,AKT或PKB)的磷酸化,促进相关基因的转录和细胞因子的产生[45]
AOS还可以通过抑制TLR4/髓样分化因子88(myeloid differentiation factor 88,MyD88)信号通路,降低促凋亡蛋白B细胞淋巴瘤-2相关X蛋白(B-cell lymphoma-2-associated X protein,Bax)和增加抗凋亡蛋白B细胞淋巴瘤-2(B-cell lymphoma-2,Bcl-2)缓解肠黏膜损伤[46]。在利用脂多糖(lipopolysaccharide,LPS)刺激巨噬细胞模型发现,AOS能够减少LPS与细胞表面结合,抑制TLR4和分化抗原CD14的表达,从而降低炎症反应发生[47]。COS可上调TLR4和核因子-κB p65亚基(nuclear factor-κB p65 subunit,NF-κB p65)的表达,抑制LPS诱导的NF-κB p65、白细胞介素-6(interleukin-6,IL-6)和白细胞介素-8(Interleukin-8,IL-8)表达,COS处理后的细胞改善了由LPS诱导的猪小肠上皮细胞系(porcine intestinal epithelial cell line,IPEC-J2细胞)的增殖率降低、上皮细胞完整性受到损害的问题[48]
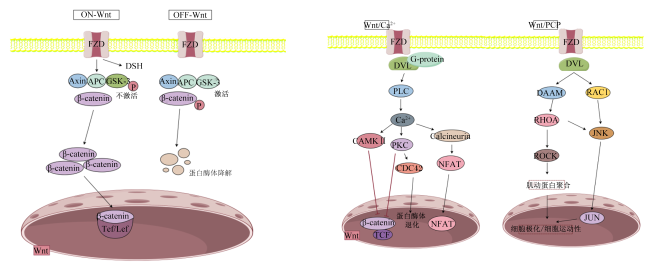
Wnt蛋白是一种分泌型糖蛋白[49],其Wnt/β-catenin信号通路是一种进化上保守的信号级联,参与细胞的增殖、分化和凋亡等过程[50]。Wnt/β-catenin信号通路也称为经典的Wnt信号通路,它的激活能导致细胞核中积累β-catenin转录组分(图2)。在不同的生物调控过程中,该经典通路有4种状态:1)经典Wnt信号通路未激活状态。此时该信号通路主要表现为腺瘤性息肉病(adenomatous polyposis coli,APC)、轴抑制蛋白(axis inhibition protein,Axin)和糖原合成酶激酶-3β(glycogen synthase kinase-3β,GSK-3β)复合物对细胞质中磷酸化β连环蛋白(p-β-catenin)的催化降解过程,在此结构中Axin是一种化合物,可影响GSK-3β和APC的结合[51],GSK-3β介导形成细胞质中p-β-catenin,随后介导其被降解[52];2)经典Wnt信号通路激活状态。当Wnt家族配体与2个共受体低密度脂蛋白受体相关蛋白(low-density lipoprotein receptor-related protein,LRP)和卷曲蛋白(frizzled,FZD)的结合时,将信号传递给细胞中的蓬乱蛋白Dsh同源物(dishevelled Dsh homolog,DVL),活化的DVL会对APC-Axin-酪蛋白激酶Ⅰ(casein kinase Ⅰ,CKⅠ)-GSK-3β复合物产生破坏作用,阻碍p-β-catenin降解,导致β-catenin在细胞质中积累,从而增强其核转位。当β-catenin进入细胞核,能够与转录因子T细胞因子/淋巴增强因子(T-cell factor/lymphoid enhancer factor,Tcf/Lef)相互作用,从而调节下游靶基因[53];3)非经典Wnt/平面细胞极性(planar cell polarity,PCP)信号通路。在该信号通路中,Wnt配体与FZD/DVL激活双调蛋白激活形态发生相关蛋白(double-homology-activated forming-associated molecule,DAAM)与Rac家族小GTP酶(Rac family small GTPase,RAC)[54],DAAM解离出Rho家族小GTP酶(Rho family small GTPase,RHOA)来激活Rho相关卷曲螺旋形成蛋白激酶(Rho-associated coiled-coil forming protein kinase,ROCK)的表达,从而影响细胞骨架的形成[55-56];DVL能够激活RAC[57],FZD6可能潜在地调节PCP和c-Jun氨基末端激酶(c-Jun N-terminal Kinase,JNK)激活,最终影响基因的转录[58];4)非典型Wnt/钙离子(Ca2+)信号通路。Wnt配体结合FZD/DVL,激活磷脂酶C(phospholipase C,PLC)并诱导细胞内Ca2+水平升高。升高的细胞内Ca2+激活钙调蛋白依赖性蛋白激酶Ⅱ(Ca2+/calmodulin-dependent protein kinase Ⅱ,CaMKⅡ)、钙调蛋白(calmodulin,CaM)和蛋白激酶C(protein kinase C,PKC),CaM能够激活活化的T细胞核内因子(nuclear factor of activated T-cells,NFAT)并促进下游靶基因的表达,PKC活化使糖原合成酶激酶-3(glycogen synthase kinase-3,GSK-3)失活来抑制β-catenin磷酸化[59]。已有研究表明,副干酪乳杆菌VL8及其与MOS的合生元组合,可以抑制葡聚糖硫酸钠(dextran sodium sulfate,DSS)诱导的Wnt/β-catenin信号通路过度激活[60];将XOS通过转谷氨酰胺酶途径与肽-钙螯合物复合,发现能有效维持胃肠道内钙含量的稳定,还可加速Caco-2细胞单层的钙转运效率,但其是否直接介导免疫细胞活化仍需进一步验证[61]
图2 Wnt信号通路(由Figdraw绘制)

FZD:卷曲蛋白 frizzled;DVL:蓬乱蛋白Dsh同源物 dishevelled Dsh homolog;Axin:轴抑制蛋白 axis inhibition protein;APC:腺瘤性息肉病 adenomatous polyposis coli;GSK-3β:糖原合成酶激酶-3β glycogen synthase kinase-3β;β-catenin:β-连环蛋白;Tcf/Lef:T细胞因子/淋巴增强因子T-cell factor/lymphoid enhancer factor;G-protein:鸟苷酸结合蛋白 guanine nucleotide-binding protein;PLC:磷脂酶C phospholipase C;CAMKⅡ:Ca2+/钙调蛋白依赖性蛋白激酶Ⅱ Ca2+/calmodulin-dependent protein kinase Ⅱ;PKC:蛋白激酶C protein kinase C;Calcineurin:钙调神经磷酸酶 calcium regulated neurophosphatase;NFAT:活化的T细胞核内因子 nuclear factor of activated T-cells;CDC42:细胞分裂周期蛋42 cell division cycle 42;DAAM:双调蛋白激活形态发生相关蛋白 double-homology-activated forming-associated molecule;RHOA:Rho家族小GTP酶A Rho family small GTPase A;ROCK:Rho相关卷曲螺旋形成蛋白激酶 Rho-associated coiled-coil forming protein kinase;RAC1:Rac家族小GTP酶1 Rac family small GTPase 1;JNK:c-Jun氨基末端激酶c-Jun N-terminal kinase;JUN:一种原癌基因 a proto-oncogene。

Fig.2 Wnt signal pathways (drawn by Figdraw)

2.3 调节炎症信号通路

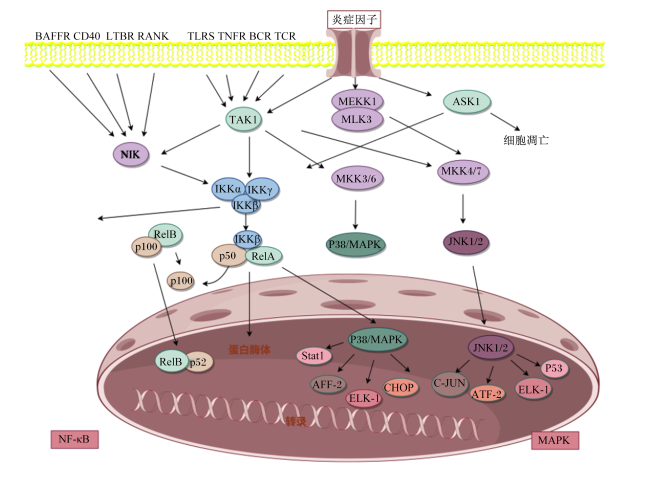
炎症调控是机体内一系列复杂的分子网络,通过感知外界刺激、激活特定的受体引发的一系列级联反应,从而影响炎症因子的释放和炎症相关基因的表达。丝裂原活化蛋白激酶(mitogen-activated protein kinase,MAPK)信号通路可调节细胞的生长、分化、凋亡和死亡等多种生理过程。生理状态下,NF-κB二聚体与κB抑制蛋白(inhibitor of κB,IκB)结合,协同抑制炎症,维持细胞生长、增殖与凋亡平衡[62]。促炎细胞因子如肿瘤坏死因子-α(tumor necrosis factor-α,TNF-α)、白细胞介素-1(interleukin-1,IL-1)、IL-6、环氧合酶-2(cyclooxygenase-2,COX-2)及诱导型一氧化氮合酶(inducible nitric oxide synthase,NOS)等激活NF-κB经典途径,刺激激活IκB激酶(IκB kinase,IKK,诱导IκB磷酸化、泛素化,释放NF-κB入核,启动靶基因转录,激活免疫细胞[63],介导免疫应答,发挥抗炎作用。MAPK位于TLR4下游信号通路,其激活涉及p38 MAPK、细胞外信号调节激酶(extracellular signal-regulated kinase,ERK)和c-Jun氨基末端激酶(C-Jun N-terminal kinase,JNK),激活后诱导激活蛋白-1(activator protein-1,AP-1)核转位,启动核内信号,释放炎症因子[64-65]。在LPS诱导的细胞炎症反应模型中,巨噬细胞识别细菌LPS等病原,引起刺激性信号传导,激活MAPK等信号通路,引发炎症性疾病[66],并调节相关基因的转录,进行一系列生物效应。
研究表明,AOS可以通过NF-κB信号通路减轻LPS诱导的瘤胃上皮细胞凋亡和炎症反应[67]。在炎症反应中,外界刺激会激活MAPK信号通路,促进炎症因子的产生和释放[68],COS可以通过调节线粒体凋亡和MAPK信号通路来减轻LPS挑战的肠道炎症[6]。橘皮素可以通过抑制MAPK信号通路,下调对NF-κB的激活,从而抑制炎症的发展[69],MAPK和NF-κB是2个在炎症反应中发挥重要作用的信号通路,它们相互作用共同调节炎症(图3)。新琼寡糖也能够通过调节MAPK和NF-κB信号通路来减弱炎症反应[70]
图3 NF-κB和MAPK信号通路(由Figdraw绘制)

BAFFR:B细胞激活因子受体 B-cell-activating factor receptor;CD40:分化簇40 cluster of differentiation 40;LTBR:淋巴毒素-β受体 lymphotoxin-β receptor;RANK:核因子-κB受体激活剂 receptor activator of nuclear factor-κB;TLRS:Toll样受体 Toll-like receptors;TNFR:肿瘤坏死因子受体 tumor necrosis factor receptor;BCR:B细胞受体 B-cell receptor;TCR:T细胞受体 T-cell receptor;TAK1:转化生长因子-β激活激酶1 transforming growth factor-β-activated kinase 1;NIK:核因子-κB诱导激酶 NF-κB-inducing kinase;IKKα:IκB激酶-α IκB kinase-α;IKKβ:IκB激酶-β IκB kinase-β;IKKγ:IκB激酶-γ IκB kinase-γ;RelB:禽网状内皮瘤病毒癌基因同源物v-relB avian reticuloendotheliosis viral oncogene homolog v-relB;MEKK1:丝裂原活化蛋白激酶/细胞外信号调节激酶激酶激酶1 mitogen-activated protein kinase/extracellular signal-regulated kinase kinase kinase 1;MLK3:混合谱系激酶3 mixed-lineage kinase 3;ASK1:细胞凋亡信号调节激酶1 apoptosis signal-regulating kinase 1;MKK3/6:丝裂原活化蛋白激酶激酶3/6 mitogen-activated protein kinase kinase 3/6;MKK4/7:丝裂原活化蛋白激酶激酶 4/7 mitogen-activated protein kinase kinase 4/7;P38/MAPK:p38丝裂原活化蛋白激酶 p38 mitogen-activated protein kinase;JNK1/2:c-Jun氨基末端激酶1/2 c-Jun N-terminal kinase 1/2;Stat1:信号转导和转录激活因子1 signal transducer and activator of transcription 1;CHOP:C/EBP同源蛋白C/EBP homologous protein;ATF-2:活化转录因子2 activating transcription factor 2;ELK-1:E74样ETS转录因子1 E74-like ETS transcription factor;NF-κB:核因子-κB nuclear factor-κB;MAPK:丝裂原活化蛋白激酶 mitogen-activated protein kinase。

Fig.3 NF-κB and MAPK signal pathways (drawn by Figdraw)

3 低聚糖在断奶仔猪饲粮中的应用

3.1 MOS对断奶仔猪的作用

Yu等[71]研究发现,饲粮中添加0.3%的MOS可以降低断奶仔猪降低腹泻率,减轻肠道损伤,改善黏膜形态与紧密连接蛋白分布,减少细胞凋亡,改善肠道结构,同时MOS能够调控基因表达,通过抑制炎症、促进抗氧化等途径维护肠道上皮功能,增强肠道局部免疫。吴中敏等[72]研究发现,饲粮中添加0.2%的MOS可促进断奶仔猪的生长,提高日增重,降低料重比,降低仔猪腹泻发生,增强细胞免疫能力以及机体抗氧化能力,提高断奶仔猪免疫性能。

3.2 AOS对断奶仔猪的作用

Wan等[73]研究发现,在基础饲粮中补充100 mg/kg的AOS可改善肠道形态与屏障功能,显著增加肠绒毛高度,能提升分泌型免疫球蛋白A含量,增强肠道局部免疫,降低肠上皮细胞总凋亡百分比,增加处于DNA合成期的细胞比例,并增加杯状细胞计数,有助于维持黏膜完整性,AOS通过上调小肠中Bcl-2转录水平,同时下调Bax、半胱天冬酶-3(Caspase-3)和半胱天冬酶-9(Caspase-9)转录水平,抑制线粒体依赖性细胞凋亡途径,进而减少肠细胞死亡,促进仔猪生长。Wan等[74]使用IPEC-J2细胞探究AOS作用机制,发现AOS能有效降低LPS与IPEC-J2细胞表面的结合,同时抑制LPS诱导的促炎细胞因子的产生以及NF-κB p65的核转位,这表明AOS通过阻止NF-κB的激活来保护肠上皮细胞免受肠毒性大肠杆菌(enterotoxigenic Escherichia coli,ETEC)诱导的炎症损伤,保护断奶仔猪肠道屏障。

3.3 FOS对断奶仔猪的作用

Ayuso等[75]研究发现,给哺乳仔猪提供1 g/d膳食短链低聚果糖(scFOS)可以改善其生长状况,也可以显著增加新生哺乳仔猪体重,降低断奶后死亡率。Luo等[76]研究发现,饲粮中添加2.5 g/kg的FOS能够提高断奶仔猪的抗氧化能力和肠道屏障的完整性,但不影响其生长性能,可以改善肠道屏障标志物的水平,降低肠黏膜中的炎性细胞因子水平,以及抑制TLR4/MyD88/NF-κB信号通路,从而减少细胞凋亡。Ferreres-Serafini等[77]研究表明,饲粮中添加5 g/kg的scFOS或1 g/kg的酿酒酵母Sc47均能显著降低断奶仔猪腹泻发生率,减少肠道中EHEC数量,有效降低断奶后大肠杆菌病的发病率,其scFOS补充主要与肠道生态系统的积极变化及乳酸杆菌数量的增加相关。Wiese等[78]使用仔猪体外结肠模型,发现FOS和GOS等可以影响总SCFAs含量,表明低聚糖可以影响仔猪的SCFAs代谢。

3.4 其他低聚糖对断奶仔猪的作用

研究发现,饲喂添加COS的断奶仔猪空肠黏膜和淋巴结中白细胞介素-1β(Interleukin-1β,IL-1β)mRNA表达水平增加,血清IL-1β、白细胞介素-2(interleukin-2,IL-2)、IL-6、免疫球蛋白A(immunoglobulin A,IgA)、免疫球蛋白G(immunoglobulin G,IgG)和免疫球蛋白M(immunoglobulin M,IgM)含量增加,COS还通过调节细胞因子和抗体的产生增强早期断奶仔猪细胞介导的免疫反应,与抗生素类似,COS增加了上皮内淋巴细胞的浓度,增加了绒毛长度、绒毛长度/隐窝深度和杯状细胞数量,降低了TLR4的mRNA表达水平,改善了免疫球蛋白特异性结合的细胞表面受体[79]。Gao等[80]研究发现,补充XOS后断奶仔猪回肠丁酸盐含量和双歧杆菌数量显著增加,回肠NF-κB蛋白表达水平降低,而MOS组回肠醋酸盐和丁酸盐含量更高;同时添加0.1%的XOS和0.08%的MOS可显著降低断奶仔猪腹泻发生率,增强肠道免疫性能,提升抗氧化能力。Wang等[81]采用2×2析因排列设计,在饲粮中添加0.43%的XOS,发现饲喂高植物蛋白质饲粮断奶仔猪的腹泻指数显著高于饲喂低植物蛋白质饲粮,表明XOS可以通过提高营养消化率减轻腹泻,保护肠道形态,优化肠道菌群。

4 小结与展望

低聚糖作为一类重要的益生元,在动物肠道内可被微生物选择性有效分解和代谢,生成SCFAs、胆汁酸等关键代谢产物,通过多途径调控肠道屏障功能并维持内环境稳态。目前,低聚糖和菌群代谢产物如何通过特定信号通路影响宿主的级联效应仍不完全明确;且现有研究多聚焦于单一低聚糖的宏观效应,缺乏对不同结构低聚糖与菌群代谢网络动态互作的组学水平解析。随着科学技术的发展,通过借助多组学技术,深入解析低聚糖与肠道、微生物及其代谢之间的分子互作网络,明确其激活或抑制关键信号通路的上下游靶点及调控级联反应,精准定位低聚糖调控肠道健康的核心通路与关键节点,开发具有靶向调控能力的新型低聚糖衍生物,将为低聚糖在绿色高效养殖中的创新应用开辟新路径,促进畜牧业可持续发展。
[1]
NIKKHAH-BODAGHI M, MALEKI I, AGAH S, et al. Zingiber officinale and oxidative stress in patients with ulcerative colitis:a randomized,placebo-controlled,clinical trial[J]. Complementary Therapies in Medicine, 2019,43:1-6.

[2]
WANG H L, CAI Y S, WU W Q, et al. Exploring the role of gut microbiome in autoimmune diseases:a comprehensive review[J]. Autoimmunity Reviews, 2024, 23(12):103654.

DOI

[3]
NAKASE H, SATO N, MIZUNO N M, et al. The influence of cytokines on the complex pathology of ulcerative colitis[J]. Autoimmunity Reviews, 2022, 21(3):103017.

DOI

[4]
LORDAN C, ROCHE A K, DELSING D, et al. Linking human milk oligosaccharide metabolism and early life gut microbiota:bifidobacteria and beyond[J]. Microbiology and Molecular Biology Reviews, 2024, 88(1):e0009423.

DOI

[5]
ZHANG E, WEI Q, LI X, et al. Effects of polymannuronic acid on the intestinal microbiota in mice after long-term intragastric administration[J]. Marine Drugs, 2024, 22(3):125.

DOI

[6]
MENG T T, LIU C M, CHEN Y L, et al. Dietary chito-oligosaccharide attenuates LPS-challenged intestinal inflammation via regulating mitochondrial apoptotic and MAPK signaling pathway[J]. International Immunopharmacology, 2024,126:111153.

[7]
CHEN C, CAO Z, LEI H H, et al. Microbial tryptophan metabolites ameliorate ovariectomy-induced bone loss by repairing intestinal AhR-mediated gut-bone signaling pathway[J]. Advanced Science, 2024, 11(36):2404545.

DOI

[8]
JANA U K, SURYAWANSHI R K, PRAJAPATI B P, et al. Prebiotic mannooligosaccharides:synthesis,characterization and bioactive properties[J]. Food Chemistry, 2021,342:128328.

[9]
XING M C, CAO Q, WANG Y, et al. Advances in research on the bioactivity of alginate oligosaccharides[J]. Marine Drugs, 2020, 18(3):144.

DOI

[10]
RASTALL R A. Functional oligosaccharides:application and manufacture[J]. Annual Review of Food Science and Technology, 2010,1:305-339.

[11]
REHMAN A U, KOVACS Z, QUITMANN H, et al. Enzymatic production of fructo oligosaccharides from inexpensive and abundant substrates using a membrane reactor system[J]. Separation Science and Technology, 2016, 51(9):1537-1545.

[12]
KULIG D, KRÓL-KILIŃSKA Ż, BOBAK Ł, et al. Functional properties of chitosan oligomers obtained by enzymatic hydrolysis[J]. Polymers, 2023, 15(18):3801.

DOI

[13]
EL-SAADONY M T, SAAD A M, ALKAFAAS S S, et al. Chitosan,derivatives,and its nanoparticles:preparation,physicochemical properties,biological activities,and biomedical applications-a comprehensive review[J]. International Journal of Biological Macromolecules, 2025,313:142832.

[14]
GUSTAFSSON J K, JOHANSSON M E V. The role of goblet cells and mucus in intestinal homeostasis[J]. Nature Reviews Gastroenterology & Hepatology, 2022, 19(12):785-803.

[15]
KUZIEL G A, RAKOFF-NAHOUM S. The gut microbiome[J]. Current Biology, 2022, 32(6):R257-R264.

[16]
GROSCHWITZ K R, HOGAN S P. Intestinal barrier function: molecular regulation and disease pathogenesis[J]. The Journal of Allergy and Clinical Immunology, 2009, 124(1):3-20.

DOI PMID

[17]
VAN DER SLUIS M, DE KONING B A E,DE BRUIJN A C J M, et al. Muc2-deficient mice spontaneously develop colitis,indicating that MUC2 is critical for colonic protection[J]. Gastroenterology, 2006, 131(1):117-129.

DOI

[18]
LUO D, LI J L, XING T, et al. Combined effects of xylo-oligosaccharides and coated sodium butyrate on growth performance,immune function,and intestinal physical barrier function of broilers[J]. Animal Science Journal, 2021, 92(1):e13545.

DOI

[19]
AGAZZI A, PERRICONE V, OMODEI ZORINI F, et al. Dietary mannan oligosaccharides modulate gut inflammatory response and improve duodenal villi height in post-weaning piglets improving feed efficiency[J]. Animals, 2020, 10(8):1283.

DOI

[20]
NA K, WEI J N, ZHANG L, et al. Effects of chitosan oligosaccharides (COS) and FMT from COS-dosed mice on intestinal barrier function and cell apoptosis[J]. Carbohydrate Polymers, 2022,297:120043.

[21]
YUAN M Y, ZHANG Z W, LIU T Y, et al. The role of nondigestible oligosaccharides in alleviating human chronic diseases by regulating the gut microbiota:a review[J]. Foods, 2024, 13(13):2157.

DOI

[22]
LI M F, DING Y Y, WEI J G, et al. Gut microbiota metabolite indole-3-acetic acid maintains intestinal epithelial homeostasis through mucin sulfation[J]. Gut Microbes, 2024, 16(1):2377576.

DOI

[23]
JIN X, JIAN Z Y, CHEN X T, et al. Short chain fatty acids prevent glyoxylate-induced calcium oxalate stones by GPR43-dependent immunomodulatory mechanism[J]. Frontiers in Immunology, 2021,12:729382.

[24]
ALONSO N, ALMER G, SEMERARO M D, et al. Impact of high-fat diet and exercise on bone and bile acid metabolism in rats[J]. Nutrients, 2024, 16(11):1744.

DOI

[25]
TSCHUCK J, THEILACKER L, ROTHENAIGNER I, et al. Farnesoid X receptor activation by bile acids suppresses lipid peroxidation and ferroptosis[J]. Nature Communications, 2023, 14(1):6908.

DOI PMID

[26]
赵凯, 程小红, 卢芬萍, 等. 基于网络药理学探讨“姜黄-虎杖”药对干预足细胞病变的作用机制[J]. 云南中医中药杂志, 2024, 45(6):60-68.

ZHAO K, CHENG X H, LU F P, et al. Based on network pharmacology,the mechanism of “turmeric-Polygonum cuspidatum” drug on the intervention of podocytic lesions was discussed[J]. Yunnan Journal of Traditional Chinese Medicine and Materia Medica, 2024, 45(6):60-68. (in Chinese)

[27]
刘潞兴, 狄鸣远, 杨强. 中药有效成分治疗骨关节炎机制中的信号通路[J]. 中国组织工程研究, 2024, 28(4):609-614.

LIU L X, DI M Y, YANG Q. Signaling pathways in the mechanism underlying active ingredients of Chinese medicine in the treatment of osteoarthritis[J]. Chinese Journal of Tissue Engineering Research, 2024, 28(4):609-614. (in Chinese)

[28]
LU Z Y, FENG L, JIANG W D, et al. Mannan oligosaccharides alleviate oxidative injury in the head kidney and spleen in grass carp (Ctenopharyngodon idella) via the Nrf2 signaling pathway after Aeromonas hydrophila infection[J]. Journal of Animal Science and Biotechnology, 2023, 14(1):58.

DOI

[29]
PAN H, FENG W J, CHEN M, et al. Alginate oligosaccharide ameliorates D-galactose-induced kidney aging in mice through activation of the Nrf2 signaling pathway[J]. BioMed Research International, 2021,2021:6623328.

[30]
WANG Y T, REN K Y, TAN J Y, et al. Alginate oligosaccharide alleviates aging-related intestinal mucosal barrier dysfunction by blocking FGF1-mediated TLR4/NF-κB p65 pathway[J]. Phytomedicine, 2023,116:154806.

[31]
ZHANG Z Y, ZHANG G, ZHANG S, et al. Fructo oligosaccharide reduces weanling pig diarrhea in conjunction with improving intestinal antioxidase activity and tight junction protein expression[J]. Nutrients, 2022, 14(3):512.

DOI

[32]
MEHMOOD T, PICHYANGKURA R, MUANPRASAT C. Chitosan oligosaccharide promotes junction barrier through modulation of PI3K/AKT and ERK signaling intricate interplay in T84 cells[J]. Polymers, 2023, 15(7):1681.

DOI

[33]
YANG Z W, HONG W L, ZHENG K, et al. Chitosan oligosaccharides alleviate H2O2-stimulated granulosa cell damage via HIF-1 α signaling pathway[J]. Oxidative Medicine and Cellular Longevity, 2022,2022:4247042.

[34]
ZHANG X X, LIANG S, GAO X H, et al. Protective effect of chitosan oligosaccharide against hydrogen peroxide-mediated oxidative damage and cell apoptosis via activating Nrf2/ARE signaling pathway[J]. Neurotoxicity Research, 2021, 39(6):1708-1720.

DOI PMID

[35]
HUANG H C, NGUYEN T, PICKETT C B. Regulation of the antioxidant response element by protein kinase C-mediated phosphorylation of NF-E2-related factor 2[J]. Proceedings of the National Academy of Sciences of the United States of America, 2000, 97(23):12475-12480.

DOI PMID

[36]
SANGHVI V R, LEIBOLD J, MINA M, et al. The oncogenic action of NRF2 depends on de-glycation by fructosamine-3-kinase[J]. Cell, 2019, 178(4):807-819.e21.

DOI PMID

[37]
MOI P, CHAN K, ASUNIS I, et al. Isolation of NF-E2-related factor 2 (Nrf2),a NF-E2-like basic leucine zipper transcriptional activator that binds to the tandem NF-E2/AP1 repeat of the beta-globin locus control region[J]. Proceedings of the National Academy of Sciences of the United States of America, 1994, 91(21):9926-9930.

[38]
赵楠楠, 李彦杰, 秦合伟, 等. 转录因子NRF2在血管性痴呆中的作用机制[J]. 生命的化学, 2023, 43(8):1286-1291.

ZHAO N N, LI Y J, QIN H W, et al. Mechanism of transcription factor NRF2 in vascular dementia[J]. Chemistry of Life, 2023, 43(8):1286-1291. (in Chinese)

[39]
MILLER A F. Superoxide dismutases:ancient enzymes and new insights[J]. FEBS Letters, 2012, 586(5):585-595.

DOI

[40]
LIM H, OH C, PARK M S, et al. Hint from an enzymatic reaction:superoxide dismutase models efficiently suppress colorectal cancer cell proliferation[J]. Journal of the American Chemical Society, 2023, 145(29):16058-16068.

DOI

[41]
LU Z Y, FENG L, JIANG W D, et al. Mannan oligosaccharides application:multipath restriction from Aeromonas hydrophila infection in the skin barrier of grass carp (Ctenopharyngodon idella)[J]. Frontiers in Immunology, 2021,12:742107.

[42]
HU K, YUAN X Z, HE H, et al. Pharmacological mechanisms of chitotriose as a redox regulator in the treatment of rat inflammatory bowel disease[J]. Biomedicine & Pharmacotherapy, 2022,150:112988.

[43]
ROPERT C. How toll-like receptors reveal monocyte plasticity:the cutting edge of antiinflammatory therapy[J]. Cellular and Molecular Life Sciences, 2019, 76(4):745-755.

DOI

[44]
UMETSU D. Cell mechanics and cell-cell recognition controls by Toll-like receptors in tissue morphogenesis and homeostasis[J]. Fly, 2022, 16(1):233-247.

DOI PMID

[45]
FANG W S, BI D C, ZHENG R J, et al. Identification and activation of TLR4-mediated signaling pathways by alginate-derived guluronate oligosaccharide in RAW264.7 macrophages[J]. Scientific Reports, 2017, 7(1):1663.

DOI

[46]
TENG Y, LI J H, GUO J, et al. Alginate oligosaccharide improves 5-fluorouracil-induced intestinal mucositis by enhancing intestinal barrier and modulating intestinal levels of butyrate and isovalerate[J]. International Journal of Biological Macromolecules, 2024, 276(Pt 1):133699.

DOI

[47]
YANG B X, LI W Z, SAEKI H, et al. Maillard-type glycated collagen with alginate oligosaccharide suppresses inflammation and oxidative stress by attenuating the expression of LPS receptors TLR4 and CD14 in macrophages[J]. Food & Function, 2024, 15(7):3629-3639.

[48]
SHI L, FANG B, YONG Y H, et al. Chitosan oligosaccharide-mediated attenuation of LPS-induced inflammation in IPEC-J2 cells is related to the TLR4/NF-κB signaling pathway[J]. Carbohydrate Polymers, 2019,219:269-279.

[49]
SHAH R, AMADOR C, CHUN S T, et al. Non-canonical Wnt signaling in the eye[J]. Progress in Retinal and Eye Research, 2023,95:101149.

[50]
ABUNA R P F, OLIVEIRA F S, LOPES H B, et al. The Wnt/β-catenin signaling pathway is regulated by titanium with nanotopography to induce osteoblast differentiation[J]. Colloids and Surfaces B:Biointerfaces, 2019,184:110513.

[51]
VON KRIES J P, WINBECK G, ASBRAND C, et al. Hot spots in beta-catenin for interactions with LEF-1,conductin and APC[J]. Natural Structural Biology, 2000, 7(9):800-807.

[52]
LI V S W, NG S S, BOERSEMA P J, et al. Wnt signaling through inhibition of β-catenin degradation in an intact Axin1 complex[J]. Cell, 2012, 149(6):1245-1256.

DOI PMID

[53]
RIM E Y, CLEVERS H, NUSSE R. The Wnt pathway:from signaling mechanisms to synthetic modulators[J]. Annual Review of Biochemistry, 2022,91:571-598.

[54]
HABAS R, KATO Y, HE X. Wnt/frizzled activation of Rho regulates vertebrate gastrulation and requires a novel forming homology protein Daam1[J]. Cell, 2001, 107(7):843-854.

DOI

[55]
MARLOW F, TOPCZEWSKI J, SEPICH D, et al. Zebrafish Rho kinase 2 acts downstream of Wnt11 to mediate cell polarity and effective convergence and extension movements[J]. Current Biology, 2002, 12(11):876-884.

DOI PMID

[56]
WINTER C G, WANG B, BALLEW A, et al. Drosophila Rho-associated kinase (Drok) links frizzled-mediated planar cell polarity signaling to the actin cytoskeleton[J]. Cell, 2001, 105(1):81-91.

DOI

[57]
HABAS R, DAWID I B, HE X. Coactivation of Rac and Rho by Wnt/frizzled signaling is required for vertebrate gastrulation[J]. Genes & Development, 2003, 17(2):295-309.

DOI

[58]
CORDA G, SALA A. Non-canonical WNT/PCP signaling in cancer:Fzd6 takes centre stage[J]. Oncogenesis, 2017, 6(7):e364.

DOI

[59]
DE A. Wnt/Ca2+ signaling pathway:a brief overview[J]. Acta Biochimica et Biophysica Sinica, 2011, 43(10):745-756.

DOI

[60]
ZHANG T, CHENG T T, GENG S, et al. Synbiotic combination between Lactobacillus paracasei VL8 and mannan-oligosaccharide repairs the intestinal barrier in the dextran sulfate sodium-induced colitis model by regulating the intestinal stem cell niche[J]. Journal of Agricultural and Food Chemistry, 2024, 72(4):2214-2228.

DOI

[61]
WU X P, WANG F F, CAI X X, et al. Characteristics and osteogenic mechanism of glycosylated peptides-calcium chelate[J]. Current Research in Food Science, 2022,5:1965-1975.

[62]
ZHANG Q, LENARDO M J, BALTIMORE D. 30 years of NF-κB:a blossoming of relevance to human pathobiology[J]. Cell, 2017, 168(1/2):37-57.

DOI

[63]
YU H, LIN L B, ZHANG Z Q, et al. Targeting NF-κB pathway for the therapy of diseases:mechanism and clinical study[J]. Signal Transduction and Targeted Therapy, 2020, 5(1):209.

DOI

[64]
ROY A, SRIVASTAVA M, SAQIB U, et al. Potential therapeutic targets for inflammation in Toll-like receptor 4 (TLR4)-mediated signaling pathways[J]. International Immunopharmacology, 2016,40:79-89.

[65]
LIU X J, YANG W P, ZHU C L, et al. Toll-like receptors and their role in neuropathic pain and migraine[J]. Molecular Brain, 2022, 15(1):73.

DOI PMID

[66]
王晶, 徐颖, 张庆. 青蒿乙素对脂多糖诱导小鼠单核巨噬细胞RAW264.7炎症反应的抑制及机制[J]. 华西药学杂志, 2021, 36(1):39-43.

WANG J, XU Y, ZHANG Q. Anti-inflammatory effect and mechanism of arteannuin B on LPS-stimulated RAW264.7 macrophages[J]. West China Journal of Pharmaceutical Sciences, 2021, 36(1):39-43. (in Chinese)

[67]
QIU X Y, YIN F Q, DU C M, et al. Alginate oligosaccharide alleviates lipopolysaccharide-induced apoptosis and inflammatory response of rumen epithelial cells through NF-κB signaling pathway[J]. Animals, 2024, 14(9):1298.

DOI

[68]
ZOU Y X, FU X T, LIU N N, et al. The synergistic anti-inflammatory activities of agaro-oligosaccharides with different degrees of polymerization[J]. Journal of Applied Phycology, 2019, 31(4):2547-2558.

DOI

[69]
SHI Y F, CHEN J X, LI S L, et al. Tangeretin suppresses osteoarthritis progression via the Nrf2/NF-κB and MAPK/NF-κB signaling pathways[J]. Phytomedicine, 2022,98:153928.

[70]
WANG W, LIU P, HAO C, et al. Neoagaro-oligosaccharide monomers inhibit inflammation in LPS-stimulated macrophages through suppression of MAPK and NF-κB pathways[J]. Scientific Reports, 2017,7:44252.

[71]
YU E, CHEN D W, YU B, et al. Amelioration of enterotoxigenic Escherichia coli-induced disruption of intestinal epithelium by manno-oligosaccharide in weaned pigs[J]. Journal of Functional Foods, 2021,82:104492.

[72]
吴中敏, 吴洪. 甘露寡糖对断奶仔猪生长性能、免疫机能及抗氧化性能的影响[J]. 中国饲料, 2024(6):5-8.

WU Z M, WU H. Effects of mannan oligosaccharides on growth performance,immune function and antioxidant performance of weaned piglets[J]. China Feed, 2024(6):5-8. (in Chinese)

[73]
WAN J, ZHANG J, CHEN D W, et al. Alginate oligosaccharide-induced intestinal morphology,barrier function and epithelium apoptosis modifications have beneficial effects on the growth performance of weaned pigs[J]. Journal of Animal Science and Biotechnology, 2018,9:58.

[74]
WAN J, ZHANG J, XU Q S, et al. Alginate oligosaccharide protects against enterotoxigenic Escherichia coli-induced porcine intestinal barrier injury[J]. Carbohydrate Polymers, 2021,270:118316.

[75]
AYUSO M, MICHIELS J, WUYTS S, et al. Short-chain fructo-oligosaccharides supplementation to suckling piglets:assessment of pre- and post-weaning performance and gut health[J]. PLoS One, 2020, 15(6):e0233910.

DOI

[76]
LUO Y H, LIU L, CHEN D W, et al. Dietary supplementation of fructo-oligosaccharides alleviates enterotoxigenic E.coli-induced disruption of intestinal epithelium in a weaned piglet model[J]. British Journal of Nutrition, 2021, 128(8):1526-1534.

DOI

[77]
FERRERES-SERAFINI L, CASTILLEJOS L, MARTÍN M, et al. Looking for possible benefits of combining short-chain fructo-oligosaccharides (scFOS) with Saccharomyces cerevisiae Sc 47 on weaned pigs orally challenged with Escherichia coli F4[J]. Animals, 2023, 13(3):526.

DOI

[78]
WIESE M, HUI Y, HOLCK J, et al. High throughput in vitro characterization of pectins for piglet nutrition[J]. Animal Microbiome, 2021, 3(1):69.

DOI

[79]
SWIATKIEWICZ S, SWIATKIEWICZ M, ARCZEWSKA-WLOSEK A, et al. Chitosan and its oligosaccharide derivatives (chito-oligosaccharides) as feed supplements in poultry and swine nutrition[J]. Journal of Animal Physiology and Animal Nutrition, 2015, 99(1):1-12.

DOI PMID

[80]
GAO H, SUN F Z, LIN G, et al. Molecular actions of different functional oligosaccharides on intestinal integrity,immune function and microbial community in weanling pigs[J]. Food & Function, 2022, 13(23):12303-12315.

[81]
WANG Q B, ZHAO Y, GUO L, et al. Xylo-oligosaccharides improve the adverse effects of plant-based proteins on weaned piglet health by maintaining the intestinal barrier and inhibiting harmful bacterial growth[J]. Frontiers in Microbiology, 2023,14:1189434.

文章导航

/