综述

植物多糖对动物肠道健康的保护作用及机制研究进展

  • 胡钰欣 , 1 ,
  • 王娟 1 ,
  • 索朗曲吉 2 ,
  • 沈留红 , 1, *
展开
  • 1 四川农业大学动物医学院, 成都 611130
  • 2 西藏阿里地区日土县农牧业综合服务管理中心, 阿里 859000
* 沈留红,教授,博士生导师,E-mail:

胡钰欣(2002—),女,山西运城人,硕士研究生,从事天然产物与兽医临床应用研究。E-mail:

Office editor: 武海龙

收稿日期: 2026-01-31

  网络出版日期: 2026-09-12

基金资助

国家自然科学基金资助项目(32473109)

四川省科学技术厅重点研发项目(2024YFFK0146)

Research Progress on Protective Effects and Mechanisms of Plant Polysaccharides on Animal Intestinal Health

  • HU Yuxin , 1 ,
  • WANG Juan 1 ,
  • Suolanquji 2 ,
  • SHEN Liuhong , 1, *
Expand
  • 1 College of Veterinary Medicine, Sichuan Agricultural University, Chengdu 611130, China
  • 2 Ritu County Agriculture and Animal Husbandry Integrated Service Management Center, Ali Prefecture, Tibet, Ali 859000, China
* professor, E-mail:

Received date: 2026-01-31

  Online published: 2026-09-12

摘要

肠道作为动物机体最大的免疫器官,在维持机体免疫稳态和防御功能中占据核心地位,然而其健康状态易受营养调控、环境应激和病原体侵袭等多重因素影响。植物天然成分在开发为动物肠道健康保护剂方面具有广泛研究和应用前景,其中植物多糖(PPs)是一类植物天然活性大分子,可与肠道菌群相互作用,通过调节肠道菌群、减轻肠道炎症、缓解肠道氧化应激、提高肠道免疫力和增强肠道屏障功能来改善动物肠道健康状态。本文综述了PPs对动物肠道健康的保护作用及机制,以期为其在健康养殖中的应用及未来的研究方向提供参考。

本文引用格式

胡钰欣 , 王娟 , 索朗曲吉 , 沈留红 . 植物多糖对动物肠道健康的保护作用及机制研究进展[J]. 动物营养学报, 2026 , 38(9) : 6456 -6464 . DOI: 10.12418/CJAN2026.517

Abstract

As the largest immune organ of the animal body, the intestine plays a central role in maintaining the body’s immune homeostasis and defense function. However, its health status is susceptible to multiple factors such as nutritional regulation, environmental stress and pathogen invasion. The plant natural ingredients have broad research and development prospects in the development of animal intestinal health protective agents. Among them, plant polysaccharides (PPs) are a kind of natural active macromolecules of a wide range of plants, which can interact with intestinal flora and improve the health status of animal intestines by regulating intestinal flora, reducing intestinal inflammation, alleviating intestinal oxidative stress, improving intestinal immunity and enhancing intestinal mucosal barrier. In this paper, the protective effects and mechanisms of PPs on animal intestinal healthy were reviewed, in order to provide theoretical basis and reference for its application in healthy breeding and its future research direction.

肠道作为动物机体核心消化器官和最大免疫器官,其健康状况直接决定动物的生长性能、抗病能力和产品品质等。炎症性肠病、渗透性腹泻、慢性便秘等肠道疾病应用氨基糖苷、氟喹诺酮、大环内酯类等抗生素治疗会引起动物机体代谢和免疫功能紊乱,常常会导致肠道菌群失衡和屏障功能受损[1-3]。为维持畜禽肠道微生态稳定和形态完整性,保证动物存活率和养殖效益,在养殖过程大量使用抗生素,结果导致病原微生物产生耐药性,进而危害人类健康。植物多糖(plant polysaccharides,PPs)是从植物的根、茎、叶、果实和副产品中通过浸提法、酶解提取法、微波辅助法或超声波法等提取而来[4-5],由葡萄糖、果糖和半乳糖等单糖通过α-或β-糖苷键按照特定比例聚合而成的植物天然活性大分子[6]。根据多糖种类的不同,可分为同多糖(由1种单糖组成,如纤维、淀粉等)和杂多糖(由多种单糖组成,如果胶和岩藻多糖等)[7],其结构与蛋白质相似,可分为一级结构(主要包括单糖的排列、组成顺序、连接方式和糖残基的组成等)和高级结构(在一级结构基础上,通过各侧链间非共价键相互作用构成更复杂的结构)[8]。越来越多研究表明,PPs可被动物机体肠道菌群降解为具有生物活性的代谢产物,这些代谢产物有促进肠道吸收[9]、调节免疫反应[9]、抗肿瘤[10]、抗氧化[11]、降糖[12]和调节肠道菌群[13-14]等生物活性,并兼具低毒副作用、生物相容性优异、可生物降解、可再生及结构多样性等特性[15]。目前,文献资料报道主要聚焦某1种或2种组合PPs对动物肠道健康研究,而缺乏PPs对动物肠道健康保护作用及机制的全面梳理总结。因此,本文从PPs减轻肠道炎症、缓解肠道氧化应激、调节肠道免疫力和增强肠道屏障功能4个方面综述了PPs在保护动物肠道健康中的作用及机制,以期为其在保护畜禽肠道健康中的进一步研究和合理应用提供参考,从而进一步提高养殖效益,推动畜牧养殖业绿色、高效和可持续发展。

1 减轻肠道炎症

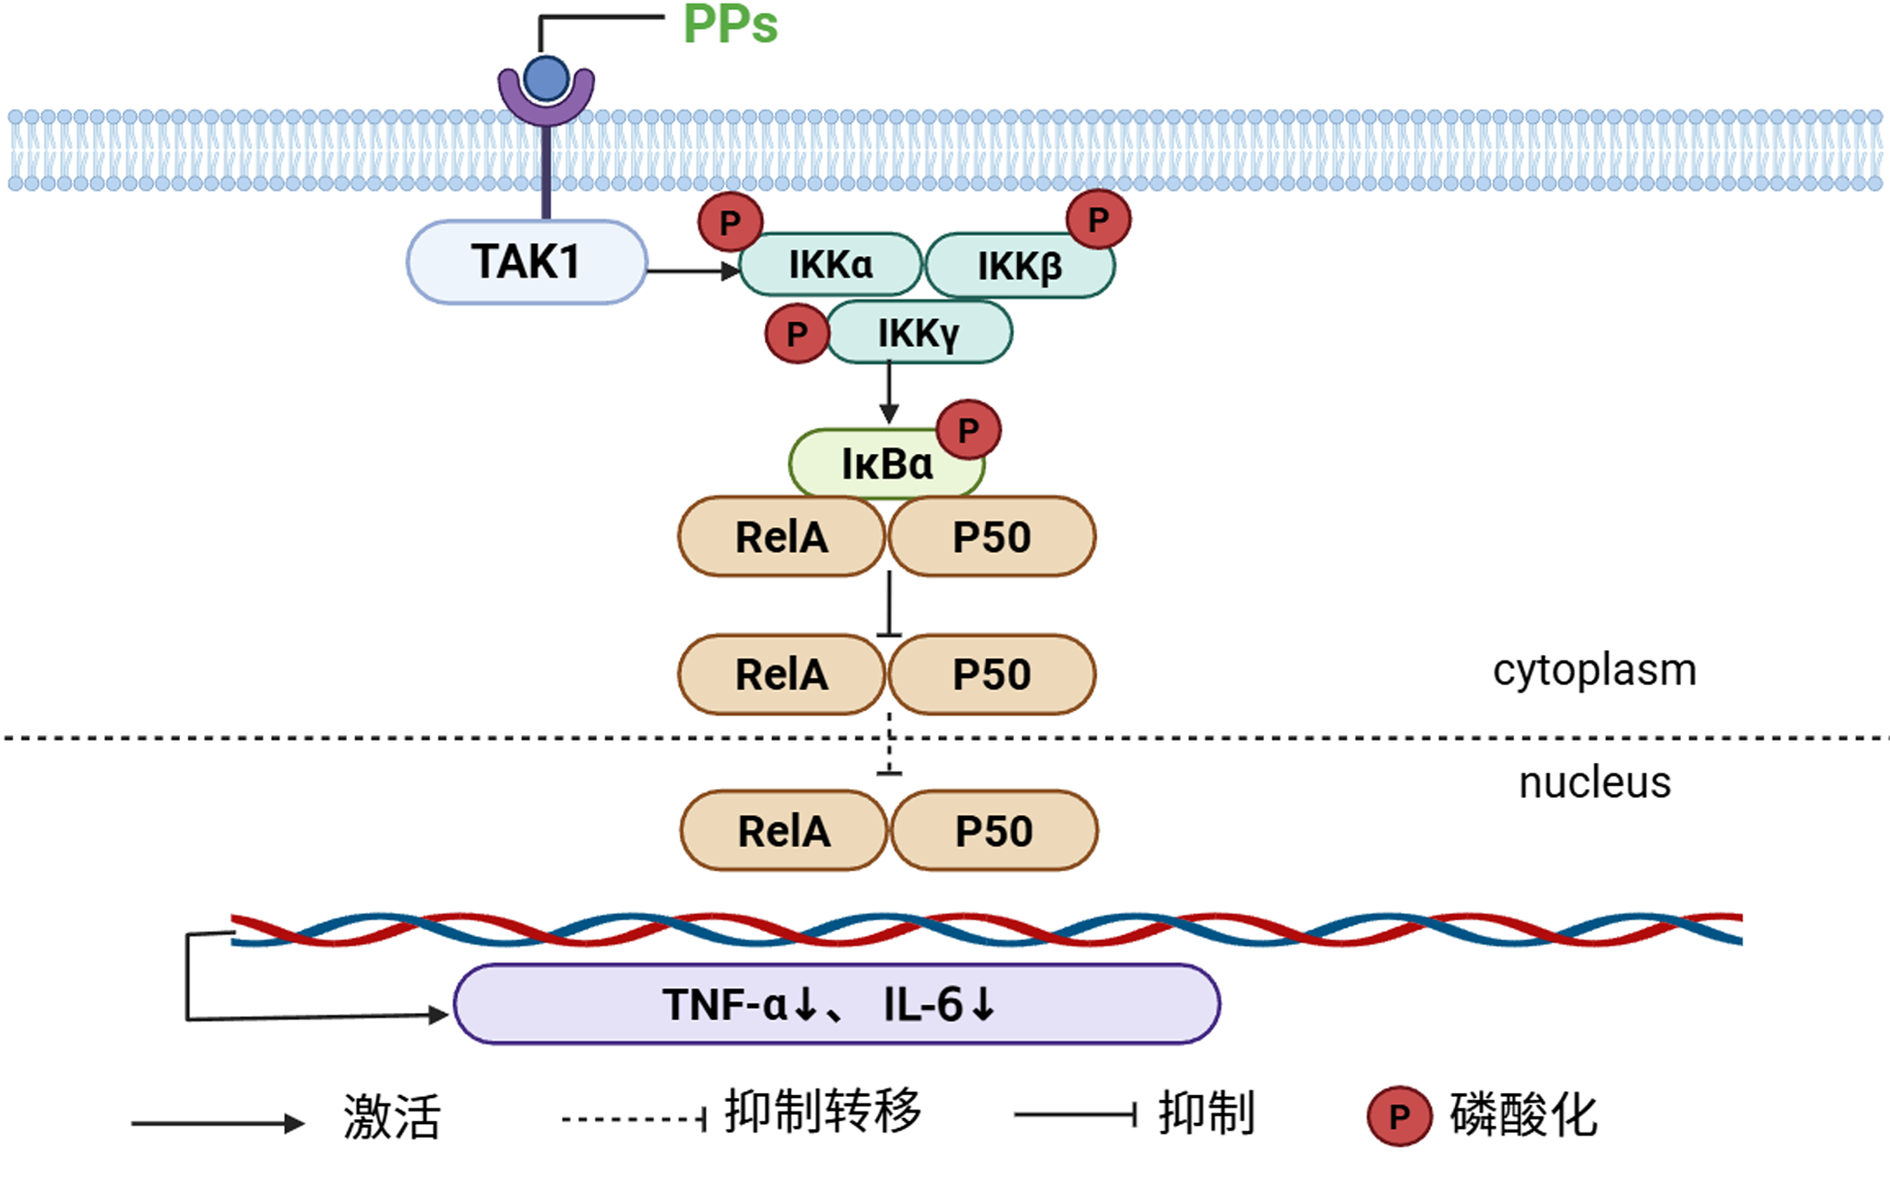
炎症是机体受病原微生物感染、损伤或代谢应激等刺激后,由先天性和/或适应性免疫介导,通过炎症细胞参与的防御和稳态修复反应,涉及体感、免疫、自主神经和血管系统的复杂生物学过程[16]。其中,促炎因子在病原体识别、免疫应答和组织修复中发挥重要作用。但是,若促炎细胞因子大量分泌,易破坏肠道菌群,损伤肠道黏膜屏障完整性,破坏肠道正常生理功能,从而引发如克罗恩病和溃疡性结肠炎等炎症性肠病,导致营养吸收受阻,影响畜禽生长速度。炎症性肠病的重要症状是肠道屏障完整性受损,若其持续存在或进一步恶化则会发展为结肠癌[17],直接增加畜禽死淘率和用药成本,导致养殖效益下降。PPs可通过抑制炎症因子分泌以减轻肠道炎症,且不易产生耐药性。研究发现,荞麦多糖可降低促炎因子白细胞介素(IL)-6、IL-1β和肿瘤坏死因子(TNF)-α分泌,从而改善2,4,6-三硝基苯磺酸诱导的大鼠结肠炎[18]。牛蒡多糖可通过抑制促炎因子IL-8、IL-6、IL-1β和TNF-α分泌治疗肠道炎症[19]。此外,辣木叶多糖可调控犊牛肠道内丝裂原活化蛋白激酶(MAPK)信号通路而抑制促炎因子分泌,减少肠道炎症的发生[20]。PPs可抑制转化生长因子β激活激酶1(TAK1)活化,阻断核因子-κB(NF-κB)抑制蛋白(IκB)激酶(IKK)复合物(IKKα/β/γ)磷酸化激活,从而抑制IκBα降解、减少NF-κB P65亚基(RelA)、NF-κB P50亚基(P50)核转移,下调TNF-αIL-6等促炎因子表达,改善结肠组织病理损伤,从而减轻肠道炎症反应[21](图1)。综上所述,PPs可通过调节NF-κB信号通路抑制促炎因子分泌来减轻肠道炎症。
图1 PPs抗炎作用机制

PPs:植物多糖 plant polysaccharides;TAK1:转化生长因子β激活激酶1 transforming growth factor beta activated kinase 1;IKK:核因子-κB抑制蛋白激酶 nuclear factor-κB inhibitor α kinase;IκBα:核因子-κB抑制蛋白α nuclear factor-κB inhibitor α;TNF-α:肿瘤坏死因子-α tumor necrosis factor-a;IL-6:白细胞介素-6 interleukin-6;RelA:NF-κB P65亚基 nuclear factor-κB P65 subunit;P50:NF-κB P50亚基 nuclear factor-κB P50 subunit;cytoplasm:细胞质;nucleus:细胞核。

Fig.1 Anti-inflammatory mechanism of PPs

2 缓解肠道氧化应激

氧化应激是由于机体氧化还原平衡被破坏,在体内积累大量自由基和氧化中间产物引起的病理生理状态[22]。氧化应激可破坏肠道微生物群,导致活性氧(ROS)生物利用度增加,从而加剧氧化应激[23],进而破坏肠道代谢[24],并形成恶性循环,造成养殖效益下降。PPs可通过改善动物机体内氧化还原酶活性和清除氧自由基以缓解肠道氧化应激。研究发现,猴头菇多糖可通过提高谷胱甘肽过氧化物酶(GSH-Px)和超氧化物歧化酶(SOD)活性,降低丙二醛(MDA)含量,缓解肠道氧化应激[25]。Zhao等[20]研究发现,辣木叶多糖可增加犊牛血清过氧化氢酶(CAT)活性和总抗氧化能力(T-AOC),降低MDA含量,防治犊牛腹泻。Yan等[26]研究发现,提取自蚊母草的果胶多糖有较强的动物肠道内自由基清除能力。由阿拉伯糖、木糖、甘露糖、葡萄糖和半乳糖组成的麦麸多糖,对动物肠道内1,1-二苯基-2-三硝基苯肼(DPPH)、2,2'-联氮双(3-乙基苯并噻唑啉-6-磺酸)二铵盐(ABTS)、羟基和超氧自由基具有较好的清除作用[27]。大麻籽多糖可通过调节核转录因子E2相关因子2(Nrf2)-Kelch样环氧氯丙烷相关蛋白1(Keap1)信号通路,增强CAT、SOD活性,从而增强肠道抗氧化能力[28]。PPs可干扰Keap1的Kelch结构域诱导Keap1构象改变,促进Nrf2脱离泛素化并核转位,与v-maf肌腱膜纤维肉瘤癌基因同源物(Maf)结合形成异二聚体后,特异性结合靶基因启动子区的抗氧化反应元件(ARE)以激活下游抗氧化相关基因转录,进而提高CAT、GSH-Px和SOD等酶类活性和T-AOC,抑制氧化应激[29](图2)。综上所述,PPs可通过调节SOD、GSH-Px和CAT等酶类活性以及清除氧自由基等方式缓解肠道氧化应激。
图2 PPs抗氧化作用机制

PPs:植物多糖 plant polysaccharides;Nrf2:核因子E2相关因子2 nuclear factor e2-related factor 2;Keap1:Kelch样环氧氯丙烷相关蛋白1 Kelch-like ECH-associated protein 1;Maf:v-maf肌腱膜纤维肉瘤癌基因同源物 v-maf fibrosarcoma oncogene homolog;ARE:抗氧化反应元件 antioxidant response elements;ROS:活性氧 reactive oxygen species;CAT:过氧化氢酶 catalase;SOD:超氧化物歧化酶 superoxide dismutase;GSH-Px:谷胱甘肽过氧化物酶 glutathione peroxidase;cytoplasm:细胞质;nucleus:细胞核。

Fig.2 Antioxidant mechanism of PPs

3 调节肠道免疫力

肠道是动物机体最大免疫器官,可构建肠道免疫屏障和调控肠道免疫应答,在调节免疫稳态中起核心作用[13]。抗生素滥用会导致肠道微生物菌群失调,进而影响免疫细胞群,削弱肠道免疫防御能力[30],导致部分炎性白细胞(中性粒细胞、单核细胞和淋巴细胞)进入肠固有层,直接或间接导致组织损伤或功能障碍,引发机体出现水肿、杯状细胞破坏、纤维化、糜烂和溃疡等症状[31],进而引起机体免疫力下降,导致畜禽对病原体易感性增强,并增加传染病传播风险,影响养殖效益。PPs可通过激活免疫细胞和调节免疫因子调节肠道免疫力。研究发现,白术多糖可减少免疫器官损伤,缓解免疫细胞(巨噬细胞、树突状细胞、T淋巴细胞和B淋巴细胞)功能下降或失衡,增强免疫反应[32]。此外,硒富集的山药糖蛋白可提高免疫抑制小鼠血清和T淋巴细胞相关的细胞因子TNF-α、IL-4、IL-6和IL-17含量,增强肠道免疫力[33-34]。人参多糖可通过RelA和MAPK P38信号通路刺激TNF-α、IL-6和一氧化氮(NO)等分泌,提升IL-2 mRNA表达水平,增强肠道免疫力[35]。Liu等[36]研究发现,黄芪多糖可促进卵清蛋白(OVA)特异性免疫球蛋白A和肠道黏膜分泌型免疫球蛋白A(sIgA)水平显著提高,增强肠道黏膜对OVA特异性免疫应答。此外,磷酸化宁氏多糖可逆转环磷酰胺诱导的胸腺和脾脏萎缩[37]。综上所述,PPs可通过激活免疫细胞和调节免疫因子从而提高肠道免疫力。

4 增强肠道屏障功能

肠道屏障是一个防止细菌和内毒素等有害物质穿透肠壁进入机体组织、器官和微循环的复杂结构,同时也吸收营养物质[38-39]。主要包括物理屏障、微生物屏障、化学屏障等,其完整性对维护肠道免受感染和机体健康至关重要。

4.1 物理屏障

物理屏障的结构主要是以紧密连接蛋白和肠上皮细胞为主,由单层紧密连接的肠道柱状上皮细胞和细胞间紧密连接构成,在调节肠道通透性方面起至关重要作用[40],若肠道上皮细胞受损会损伤肠道屏障并增加其通透性[41]。完整的肠道形态是肠道正常消化和吸收的前提,肠道绒毛高度(VH)、隐窝深度(CD)和绒隐比(V/C)是反映肠道生理形态及功能状态的重要指标,VH越高,CD越浅,肠道消化吸收营养物质能力越强[42-43]。Xie等[44]研究发现,人参多糖可增加雪峰黑骨鸡VH,减少CD,进而改善肠道黏膜屏障结构,维护肠道健康。闭合蛋白-1(Claudin-1)、咬合蛋白(Occludin)和闭锁小带蛋白-1(ZO-1)含量是评价肠上皮细胞物理屏障功能重要指标。研究发现,茯苓多糖可显著上调肉鸡十二指肠Occludin以及空肠Claudin-1、OccludinZO-1的mRNA表达[45]。猴头菇多糖和桃胶多糖可增加肠道ZO-1的mRNA表达水平,维持肠道黏膜完整性,从而增强肠道物理屏障[25,46]。人参多糖可增加肠道ZO-1和Occludin的蛋白表达水平,减轻右旋糖酐硫酸钠诱发的结肠炎[47]。二胺氧化酶(DAO)是由肠道绒毛上皮细胞分泌的细胞内酶,其血清活性可一定程度反映肠道黏膜损伤水平。D-乳酸(D-LA)是一种肠道微生物代谢产物,若肠道屏障功能受损,其可进入全身循环[48]。研究表明,黄芪多糖和甘草多糖可降低家禽肠道黏膜DAO活性,有助于肠道屏障功能恢复[49]。综上所述,PPs可通过提高VH与降低CD和增加Claudin-1、Occludin与ZO-1含量以及增强DAO活性等改善肠道物理屏障,进而增强肠道屏障功能。

4.2 微生物屏障

微生物屏障由肠道黏膜层菌群组成,其不仅可通过争夺有限的营养物质和释放抗菌物质以抑制病原体增殖,且可促进宿主体内的多种生理过程[42]。肠道菌群是一个复杂微生物群落,在正常机体中,有益菌和有害菌之间保持平衡关系,共同维持肠道健康[50]。但是,当肠道菌群失衡后会破坏机体肠道屏障功能和免疫调节功能,引起炎症性肠病、结肠癌和肠易激综合征等肠道疾病[51-53]。PPs可选择性促进有益菌生长,抑制有害菌生长[54]。鱼腥草多糖与植物乳杆菌P101组合可增加拟普雷沃氏菌属(Alloprevotella)、罗斯氏菌属(Roseburia)和嗜黏蛋白阿克曼菌(Akkermansia muciniphila)等有益菌相对丰度,降低另枝菌属(Alistipes)、肠杆状菌属(Enterorhabdus)、厌氧棍状菌属(Anaerotruncus)和埃希氏-志贺氏菌属(Escherichia-Shigella)等有害菌相对丰度,减轻肠道炎症[55]。同时,石斛多糖可通过增强罗姆布茨菌属(Romboutsia)、乳杆菌属(Lactobacillus)和臭杆菌属(Odoribacter)相对丰度以及减少副萨特氏菌属(Parasutterella)、伯尔霍尔德菌属(Burkholderia)和不动杆菌属(Acinetobacter)相对丰度以调节结肠炎肠道微生物群组成和新陈代谢[56]。PPs通常不被机体直接消化吸收,而是被肠道微生物降解为有生物活性的代谢产物,如丁酸盐和丙酸盐等短链脂肪酸(SCFAs)[54]。SCFAs可刺激肠道上皮细胞增殖和分化,增加绒毛高度,从而增加吸收表面积[42]。SCFAs还可抑制大肠杆菌、沙门氏菌和志贺氏菌等病原菌在肠道定植,进而保护肠道健康[57]。综上所述,PPs可通过增加有益菌相对丰度、降低有害菌相对丰度、提升SCFAs含量来改善肠道微生物屏障,进而增强肠道屏障功能。

4.3 化学屏障

化学屏障由消化酶、糖蛋白、黏蛋白和抑菌物质等组成,在维持肠道屏障功能和稳态方面发挥重要作用[58],若其受损会导致肠道黏液层变薄,细菌毒素、未消化的食物大分子或病原体等可穿过屏障进入体内[59]。肠道消化酶(如淀粉酶、蛋白酶、脂肪酶等)可将食物大分子分解为小分子营养物质,为肠上皮细胞提供能量和营养,保障肠道黏膜修复和更新能力。但是,当其紊乱时会诱发肠道菌群失衡,导致有害菌过度增殖,释放炎症介质,加重肠道黏膜充血、水肿[60]。王嘉麟等[61]研究发现,岩藻多糖可使羔羊空肠α-淀粉酶、脂肪酶、胰蛋白酶和糜蛋白酶活性增强。黏蛋白2(MUC2)是肠黏液层重要组成部分,当不利因素引起肠黏膜损伤或MUC2缺乏时会导致病菌直接与肠黏液层接触,从而发生自发性结肠炎[62]。研究表明,菊粉多糖能够促进感染大肠杆菌仔猪回肠MUC2基因表达水平显著升高,以保护肠黏膜[63]。肠道抑菌肽主要由肠上皮细胞和潘氏细胞分泌,可通过破坏病原菌细胞膜、抑制核酸或蛋白质合成抵御病原菌入侵,也可通过上调紧密连接蛋白表达,减少肠上皮细胞凋亡和保护肠道黏膜完整性[64]。当其分泌不足或活性异常时会导致肠黏膜通透性升高,肠道屏障功能受损,引发炎症性肠病、结肠癌等疾病[65]。研究表明,香菇多糖可激活C型凝集素-1(Dectin-1)-3型先天性淋巴细胞(ILC3)-IL-22信号轴,上调抗菌肽再生胰岛衍生蛋白3γ(REG3γ)表达,同时上调肠道MUC2和岩藻糖基转移酶表达[66]。果胶多糖通过调控肠道菌群色氨酸代谢物-芳香烃受体(AhR)-IL-22信号通路,促进ILC3分泌IL-22,激活信号转导和转录激活因子3(STAT3)磷酸化,进而增强肠道抗菌肽和黏蛋白表达[67]。综上所述,PPs可通过增强肠道消化酶与抑菌肽活性和增加MUC2含量,改善肠道化学屏障,进而增强肠道屏障功能。
综上所述,PPs可通过物理屏障、微生物屏障、化学屏障来增强肠道屏障功能,但其对各屏障间的作用机制是否存在协同作用尚需进一步研究。

5 小结与展望

PPs可通过调节NF-κB信号通路抑制促炎因子分泌减轻肠道炎症,调节SOD、GSH-Px和CAT等酶类的活性以及清除氧自由基等方式缓解肠道氧化应激,激活免疫细胞和免疫因子调节肠道免疫力,提高VH与降低CD和增加Claudin-1、Occludin与ZO-1的含量以及增强DAO活性,增加有益菌相对丰度、降低有害菌相对丰度、提升SCFAs含量,增强肠道消化酶与抑菌肽活性、增加MUC2含量增强肠道屏障功能等多重机制,在保护动物肠道健康方面发挥重要作用。尽管已有显著研究进展,但其大数侧重于单一多糖的效应研究,构效关系也不明晰,且缺乏对不同来源、结构的PPs综合利用研究。未来可借助人工智能辅助分析PPs精准结构,挖掘更多新型天然多糖资源及其关键调控靶点,并通过制剂技术提升多糖生物利用度,以实现畜牧养殖业中更广泛的应用,减少抗生素使用,助力养殖业绿色可持续发展。
[1]
MENG X, ZHANG G, CAO H, et al. Gut dysbacteriosis and intestinal disease:mechanism and treatment[J]. Journal of Applied Microbiology, 2020, 129(4):787-805.

DOI

[2]
ZHANG Y F, XUE G G, WANG F, et al. The impact of antibiotic exposure on antibiotic resistance gene dynamics in the gut microbiota of inflammatory bowel disease patients[J]. Frontiers in Microbiology, 2024, 15:1382332.

DOI

[3]
WANG M, FU R J, XU D Q, et al. Traditional Chinese medicine:a promising strategy to regulate the imbalance of bacterial flora,impaired intestinal barrier and immune function attributed to ulcerative colitis through intestinal microecology[J]. Journal of Ethnopharmacology, 2024, 318(Pt A):116879.

[4]
ZHOU Y, CHEN X X, CHEN T T, et al. A review of the antibacterial activity and mechanisms of plant polysaccharides[J]. Trends in Food Science & Technology, 2022, 123:264-280.

[5]
LI P L, HE W S, YAO H M, et al. Preparation,structural analysis,antitumor mechanism and research in drug delivery systems of natural plant polysaccharides:a review[J]. Carbohydrate Polymer Technologies and Applications, 2025, 11:100957.

DOI

[6]
YU Y, SHEN M Y, SONG Q Q, et al. Biological activities and pharmaceutical applications of polysaccharide from natural resources:a review[J]. Carbohydrate Polymers, 2018, 183:91-101.

DOI

[7]
郑伟剑, 黄东璋, 王郡东, 等. 植物多糖在肉鸡生产中的应用研究进展[J]. 动物营养学报, 2026, 38(1):58-67.

DOI

ZHENG W J, HUANG D Z, WANG J D, et al. Research progress on application of plant polysaccharides in broiler production[J]. Chinese Journal of Animal Nutrition, 2026, 38(1):58-67. (in Chinese)

DOI

[8]
于向宇, 张桂杰, 陈晓东. 植物多糖生物活性及其在反刍动物生产中应用的研究进展[J]. 中国畜牧兽医, 2025, 52(6):2626-2636.

DOI

YU X Y, ZHANG G J, CHEN X D. Research progress on biological activities of plant polysaccharides and their application in ruminant production[J]. China Animal Husbandry & Veterinary Medicine, 2025, 52(6):2626-2636. (in Chinese)

[9]
XIAO W W, ZHOU P F, WANG X S, et al. Comparative characterization and immunomodulatory activities of polysaccharides extracted from the radix of Platycodon grandiflorum with different extraction methods[J]. Molecules, 2022, 27(15):4759.

DOI

[10]
HE X Y, WANG Z, XIAO Y, et al. Gynostemma pentaphyllum polysaccharide prevents the growth of h22 ascites tumour by enhancing immunity rather than cytotoxicity in mice[J]. Food and Agricultural Immunology, 2020, 31(1):367-378.

DOI

[11]
LIU S L, WANG L T, REN Q, et al. Immunomodulatory and antioxidant activities of a polysaccharide from Ligustrum vicaryi L. fruit[J]. Evidence-Based Complementary and Alternative Medicine, 2020,2020(1):5431350.

[12]
WANG H T, LI H L, HOU Y T, et al. Plant polysaccharides:sources,structures,and antidiabetic effects[J]. Current Opinion in Food Science, 2023, 51:101013.

DOI

[13]
TAKIISHI T, FENERO C I M, CÂMARA N O S. Intestinal barrier and gut microbiota:shaping our immune responses throughout life[J]. Tissue Barriers, 2017, 5(4):e1373208.

DOI

[14]
XUE H K, TANG Y Q, ZHA M, et al. The structure-function relationships and interaction between polysaccharides and intestinal microbiota:a review[J]. International Journal of Biological Macromolecules, 2025, 291:139063.

DOI

[15]
ZHAO H H, LI Q Y, SHI A H, et al. Application of plant polysaccharide nanoparticles as polymeric carrier materials for the construction of medicine carriers[J]. Journal of Cluster Science, 2023, 34(5):2215-2228.

DOI

[16]
MATSUDA M, HUH Y, JI R R. Roles of inflammation,neurogenic inflammation,and neuroinflammation in pain[J]. Journal of Anesthesia, 2019, 33(1):131-139.

DOI

[17]
LANDY J, RONDE E, ENGLISH N, et al. Tight junctions in inflammatory bowel diseases and inflammatory bowel disease associated colorectal cancer[J]. World Journal of Gastroenterology, 2016, 22(11):3117-3126.

DOI PMID

[18]
YANG J Y, CHEN S Y, WU Y H, et al. Ameliorative effect of buckwheat polysaccharides on colitis via regulation of the gut microbiota[J]. International Journal of Biological Macromolecules, 2023, 227:872-883.

DOI

[19]
ZENG F, LI Y, ZHANG X X, et al. Immune regulation and inflammation inhibition of Arctium lappa L. polysaccharides by TLR4/NF-κB signaling pathway in cells[J]. International Journal of Biological Macromolecules, 2024, 254(Pt 2):127700.

DOI

[20]
ZHAO C, LI H F, GAO C Y, et al. Moringa oleifera leaf polysaccharide regulates fecal microbiota and colonic transcriptome in calves[J]. International Journal of Biological Macromolecules, 2023, 253(Pt 6):127108.

DOI

[21]
WANG Z, WANG L, WU X, et al. Polysaccharide extracted from Portulacae oleracea L. exerts protective effects against dextran sulfate sodium-induced colitis through inhibition of NF-κB[J]. American Journal of Translational Research, 2018, 10(8):2502-2510.

[22]
YANG Z, MAN J Y, LIU H Y, et al. Study on the in vitro and in vivo antioxidant activity and potential mechanism of Polygonum viviparum L.[J]. Antioxidants, 2025, 14(1):41.

DOI

[23]
SUN Y Q, WANG X R, LI L, et al. The role of gut microbiota in intestinal disease:from an oxidative stress perspective[J]. Frontiers in Microbiology, 2024, 15:1328324.

DOI

[24]
WANG X F, CHEN X, TANG Y, et al. The therapeutic potential of plant polysaccharides in metabolic diseases[J]. Pharmaceuticals, 2022, 15(11):1329.

DOI

[25]
TIAN B M, WANG P Y, XU T R, et al. Ameliorating effects of Hericium erinaceus polysaccharides on intestinal barrier injury in immunocompromised mice induced by cyclophosphamide[J]. Food & Function, 2023, 14(6):2921-2932.

[26]
YAN S, LIU X B, WANG Y W, et al. Structural characterization and antioxidant activity of pectic polysaccharides from Veronica peregrina L.[J]. Frontiers in Nutrition, 2023, 10:1217862.

DOI

[27]
SHANG X L, LIU C Y, DONG H Y, et al.Extraction, purification,structural characterization,and antioxidant activity of polysaccharides from wheat bran[J]. Journal of Molecular Structure, 2021, 1233:130096.

DOI

[28]
WEN Z S, XUE R, DU M, et al. Hemp seed polysaccharides protect intestinal epithelial cells from hydrogen peroxide-induced oxidative stress[J]. International Journal of Biological Macromolecules, 2019, 135:203-211.

DOI

[29]
CHEN N, HU M F, JIANG T Y, et al. Insights into the molecular mechanisms,structure-activity relationships and application prospects of polysaccharides by regulating Nrf2-mediated antioxidant response[J]. Carbohydrate Polymers, 2024, 333:122003.

DOI

[30]
ZHANG S, CHEN D C. Facing a new challenge:the adverse effects of antibiotics on gut microbiota and host immunity[J]. Chinese Medical Journal, 2019, 132(10):1135-1138.

DOI

[31]
TANG M S, CHENG L, LIU Y N, et al. Plant polysaccharides modulate immune function via the gut microbiome and may have potential in COVID-19 therapy[J]. Molecules, 2022, 27(9):2773.

DOI

[32]
ZHAO R H, YANG F X, BAI Y C, et al. Research progress on the mechanisms underlying poultry immune regulation by plant polysaccharides[J]. Frontiers in Veterinary Science, 2023, 10:1175848.

DOI

[33]
WANG S Q, YU J J, ZHOU L L, et al. Glycoprotein from selenium-enriched yam activates immune cells and enhances intestinal immunity via the NF-κB signaling pathway[J]. Food Bioscience, 2024, 61:104671.

DOI

[34]
XU L Y, BOTCHWAY B O A, ZHANG S O, et al. Inhibition of NF-κB signaling pathway by resveratrol improves spinal cord injury[J]. Frontiers in Neuroscience, 2018, 12:690.

DOI PMID

[35]
GHOSH R, BRYANT D L, ARIVETT B A, et al. An acidic polysaccharide (AGC3) isolated from North American ginseng (Panax quinquefolius) suspension culture as a potential immunomodulatory nutraceutical[J]. Current Research in Food Science, 2020, 3:207-216.

DOI

[36]
LIU C, LUO J, XUE R Y, et al. The mucosal adjuvant effect of plant polysaccharides for induction of protective immunity against Helicobacter pylori infection[J]. Vaccine, 2019, 37(8):1053-1061.

DOI

[37]
HUANG L F, WANG J N, WANG L T, et al. Phosphorylated Scrophularia ningpoensis polysaccharides mitigate oxidative stress and modulate immunity by regulating the gut microbiota in cyclophosphamide-treated mice[J]. Food Bioscience, 2025, 72:107463.

DOI

[38]
GOU H Z, ZHANG Y L, REN L F, et al. How do intestinal probiotics restore the intestinal barrier?[J]. Frontiers in Microbiology, 2022, 13:929346.

DOI

[39]
SYLVESTRE M. DI CARLO S E, PEDUTO L. Stromal regulation of the intestinal barrier[J]. Mucosal Immunology, 2023, 16(2):221-231.

DOI

[40]
李新科, 杨雪, 张萱, 等. 短链脂肪酸对肠道屏障保护作用的研究进展[J]. 动物营养学报, 2024, 36(8):4861-4871.

DOI

LI X K, YANG X, ZHANG X, et al. Research progress on protective effects of short chain fatty acids on intestinal barrier[J]. Chinese Journal of Animal Nutrition, 2024, 36(8):4861-4871. (in Chinese)

DOI

[41]
WANG S Q, LI H H, DU C H, et al. Effects of dietary supplementation with Lactobacillus acidophilus on the performance,intestinal physical barrier function,and the expression of NOD-like receptors in weaned piglets[J]. PeerJ, 2018, 6:e6060.

DOI

[42]
GUO S W, XING Y Y, XU Y Q, et al. Progress of studies on plant-derived polysaccharides affecting intestinal barrier function in poultry[J]. Animals, 2022, 12(22):3205.

DOI

[43]
张泽茹, 赵玉全, 董可, 等. 植物提取物促动物生长作用机制的研究进展[J]. 动物营养学报, 2023, 35(8):4850-4859.

DOI

ZHANG Z R, ZHAO Y Q, DONG K, et al. Research progress on mechanism of action of plant extracts to promote animal growth[J]. Chinese Journal of Animal Nutrition, 2023, 35(8):4850-4859. (in Chinese)

DOI

[44]
XIE Y Q, LIU J, WANG H, et al. Effects of fermented feeds and ginseng polysaccharides on the intestinal morphology and microbiota composition of Xuefeng black-bone chicken[J]. PLoS One, 2020, 15(8):e0237357.

DOI

[45]
ZHANG J Z, ZHANG Y T, WANG Y Y, et al. Research note:Poria cocos polysaccharide alleviates lipopolysaccharide-induced intestinal inflammation and barrier damage in broiler chickens[J]. Poultry Science, 2024, 103(10):104126.

DOI

[46]
LI S G, LI G P, LIU D J, et al. Peach gum polysaccharide protects intestinal barrier function,reduces inflammation and oxidative stress,and alleviates pulmonary inflammation induced by Enterococcus faecium E745[J]. Journal of Functional Foods, 2024, 115:106098.

DOI

[47]
LI S S, HUO X H, QI Y L, et al. The protective effects of ginseng polysaccharides and their effective subfraction against dextran sodium sulfate-induced colitis[J]. Foods, 2022, 11(6):890.

DOI

[48]
LYU S C, ZHONG G Q, SHI R J, et al. Diamine oxidase as a biomarker for depression and disease activity in inflammatory bowel disease:a cross-sectional observational study[J]. World Journal of Psychiatry, 2025, 15(8):106971.

[49]
WAN X H, YIN Y M, ZHOU C Z, et al. Polysaccharides derived from Chinese medicinal herbs:a promising choice of vaccine adjuvants[J]. Carbohydrate Polymers, 2022, 276:118739.

DOI

[50]
FENG W W, AO H, PENG C, et al. Gut microbiota,a new frontier to understand traditional Chinese medicines[J]. Pharmacological Research, 2019, 142:176-191.

DOI

[51]
NIU W, YANG F Y, FU Z W, et al. The role of enteric dysbacteriosis and modulation of gut microbiota in the treatment of inflammatory bowel disease[J]. Microbial Pathogenesis, 2022, 165:105381.

DOI

[52]
RAY D, KIDANE D. Gut microbiota imbalance and base excision repair dynamics in colon cancer[J]. Journal of Cancer, 2016, 7(11):1421-1430.

DOI PMID

[53]
WU Y H, LI Y T, ZHENG Q, et al. The efficacy of probiotics,prebiotics,synbiotics,and fecal microbiota transplantation in irritable bowel syndrome:a systematic review and network meta-analysis[J]. Nutrients, 2024, 16(13):2114.

DOI

[54]
ZHANG L, CHEN X, LI J L, et al. Natural plant polysaccharides drive multidimensional metabolic homeostasis via the “gut microbiota-metabolite-host” axis[J]. International Journal of Biological Macromolecules, 2025, 329(Pt 1):147728.

DOI

[55]
XU X W, LIU S J, ZHAO Y, et al. Combination of Houttuynia cordata polysaccharide and Lactiplantibacillus plantarum P101 alleviates acute liver injury by regulating gut microbiota in mice[J]. Journal of the Science of Food and Agriculture, 2022, 102(15):6848-6857.

DOI

[56]
WANG Y J, LI Q M, ZHA X Q, et al. Dendrobium fimbriatum hook polysaccharide ameliorates dextran-sodium-sulfate-induced colitis in mice via improving intestinal barrier function,modulating intestinal microbiota,and reducing oxidative stress and inflammatory responses[J]. Food & Function, 2022, 13(1):143-160.

[57]
FUKUDA S, TOH H, HASE K, et al. Bifidobacteria can protect from enteropathogenic infection through production of acetate[J]. Nature, 2011, 469(7331):543-547.

DOI

[58]
YE Y R, ZE L C, DUAN M Q, et al. Protective effects of plant polysaccharides on intestinal health via targeted regulation of gut microbiota[J]. Journal of the Science of Food and Agriculture, 2025, 105(15):8346-8358.

DOI

[59]
MACURA B, KIECKA A, SZCZEPANIK M. Intestinal permeability disturbances:causes,diseases and therapy[J]. Clinical and Experimental Medicine, 2024, 24(1):232.

DOI

[60]
LUSHCHAK V I. Symphony of digestion:coordinated host-microbiome enzymatic interplay in gut ecosystem[J]. Biomolecules, 2025, 15(8):1151.

DOI

[61]
王嘉麟, 吴鹏鑫, 王胜男, 等. 饲粮中添加岩藻多糖对羔羊生长性能、肠道消化酶活性和微生物区系的影响[J]. 动物营养学报, 2023, 35(4):2417-2430.

DOI

WANG J L, WU P X, WANG S N, et al. Effects of dietary fucoidan on growth performance,intestinal digestive enzyme activities and microbial flora of lambs[J]. Chinese Journal of Animal Nutrition, 2023, 35(4):2417-2430. (in Chinese)

[62]
YE J Y, HASKEY N, DADLANI H, et al. Deletion of mucin 2 induces colitis with concomitant metabolic abnormalities in mice[J]. American Journal of Physiology:Gastrointestinal and Liver Physiology, 2021, 320(5):G791-G803.

[63]
ŚWIECH E, BARSZCZ M, TACIAK M, et al. Mucin gene expression in the large intestine of young pigs:the effect of dietary level of two types of chicory inulin[J]. Nutrition, 2025, 131:112635.

DOI

[64]
李梁岚, 李维勤. 潘氏细胞及其分泌的抗菌肽与肠道功能稳定和疾病的关系[J]. 中国细胞生物学学报, 2024, 46(10):1801-1809.

LI L L, LI W Q. Paneth cells and the antimicrobial peptides secreted by them:link to intestinal stability and diseases[J]. Chinese Journal of Cell Biology, 2024, 46(10):1801-1809. (in Chinese)

[65]
KIM J M. Antimicrobial proteins in intestine and inflammatory bowel diseases[J]. Intestinal Research, 2014, 12(1):20-33.

DOI PMID

[66]
ZHANG Y, ZHOU Z H, ZHANG Z M, et al. Lentinan mitigates ulcerative colitis via the IL-22 pathway to repair the compromised mucosal barrier and enhance antimicrobial defense[J]. International Journal of Biological Macromolecules, 2025, 307(Pt 1):141784.

DOI

[67]
DANG G Q, WEN X B, ZHONG R Q, et al. Pectin modulates intestinal immunity in a pig model via regulating the gut microbiota-derived tryptophan metabolite-AhR-IL22 pathway[J]. Journal of Animal Science and Biotechnology, 2023, 14(4):1451-1465.

文章导航

/