综述

围产期补饲过瘤胃蛋氨酸对幼龄反刍动物生长发育的影响及调控机制研究进展

  • 付琳 ,
  • 张丽 ,
  • 王琳 ,
  • 董贤文 , *
展开
  • 重庆市畜牧科学院,荣昌 402460
* 董贤文,副研究员,E-mail:

付 琳(1990—),女,河南三门峡人,助理研究员,硕士,主要从事反刍动物营养研究。E-mail:

收稿日期: 2022-06-12

  网络出版日期: 2023-01-11

基金资助

国家自然科学基金青年科学基金(32002206)

重庆市自然科学基金重点项目(cst2020jcyj-zdxmX0005)

重庆市博士后科研项目特别资助(XmT2018001)

Research Progress of Effects of Maternal Supplementing Rumen-Protected Methionine during Transition Period on Growth and Development of Young Ruminant and Regulatory Mechanism

  • FU Lin ,
  • ZHANG Li ,
  • WANG Lin ,
  • DONG Xianwen , *
Expand
  • Chongqing Academy of Animal Sciences, Rongchang 402460, China
* associate professor, E-mail:

Received date: 2022-06-12

  Online published: 2023-01-11

摘要

围产期是反刍动物重要的生理阶段,研究发现反刍动物围产期补饲过瘤胃蛋氨酸(RPM)不仅对母体具有显著的营养调控作用,对幼畜的生长发育、机体健康和产品品质等也有重要影响。因此,本文从RPM的营养调控功能,围产期补饲RPM调控母体、胎儿后期及幼龄阶段的影响及调控机制进行综述,以期进一步为反刍动物围产期营养调控研究提供理论依据。

本文引用格式

付琳 , 张丽 , 王琳 , 董贤文 . 围产期补饲过瘤胃蛋氨酸对幼龄反刍动物生长发育的影响及调控机制研究进展[J]. 动物营养学报, 2023 , 35(1) : 31 -42 . DOI: 10.3969/j.issn.1006-267x.2023.01.004

Abstract

The transition period is an important physiological stage for ruminants. Current study found that supplementation of rumen-protected methionine during the transition period of ruminant not only has a significant nutritional regulation effect on the mother, but also has a significant effect on the growth and development, body health and product quality of their kids. Therefore, this paper reviewed related to the effects and mechanism of supplementing rumen-protected methionine during the transition period of ruminant on the maternal, late fetal and early ruminants, in order to provide a theoretical basis for the research on transition nutritional regulation of ruminants.

幼龄反刍动物作为成年家畜的后备群体,其培育效果极大地影响反刍动物群体数量、生产性能和产品质量,幼龄反刍动物的科学培育是保证牛羊养殖业稳步发展的关键环节之一。幼龄反刍动物的培育开始于母体妊娠,并且贯穿于整个妊娠周期,直至成年。围产期为产前21 d至产后21 d,其是母体妊娠、分娩和哺育幼畜的重要过渡生理阶段。围产前期(产前21 d至分娩)是母体妊娠的最后阶段,同时该期胎儿迅速生长,对母体营养及代谢状况极其敏感,易受到母体营养变化的影响。围产后期(分娩至产后21 d)是母体的产后阶段,该期母体因分娩采食量降低,同时因哺乳而营养需求增加,极易导致能量负平衡,从而影响母乳营养水平,影响幼龄反刍动物的健康和生长发育。因此,针对围产期反刍动物母体的营养调控,通过改善母体健康状况和泌乳性能,会极大影响胎儿末期的宫内生长和出生后幼龄阶段的生长发育[1]
过瘤胃蛋氨酸(rumen protected methionine,RPM)作为一种氨基酸添加剂,在促进反刍动物生产、提高饲料利用效率及减缓蛋白质饲料资源紧张等方面起到了积极作用。RPM被广泛用于奶牛围产期营养调控。研究显示,饲粮中添加RPM是改善反刍动物母体围产期能量负平衡、保障机体健康和提高产后泌乳性能的有效途径[2-4]。此外,围产期间对母体补饲RPM能影响胎儿后期的发育,并且对幼龄反刍动物机体代谢、免疫机能、消化道微生物组成、生长性能及产品品质等具有调控作用[5-9]。这些研究表明,反刍动物围产期间补饲RPM可以通过调控母体机体代谢,进而影响后代的生长发育。但是,目前针对围产期母体补饲RPM调控反刍动物后代生理状态和生长发育的研究较少,且系统性不强。
因此,本文将以反刍动物幼畜的生理健康调控为核心,从RPM的营养调控作用、围产期补饲RPM对幼龄反刍动物的影响和围产期补饲RPM对幼龄反刍动物生长发育调控机制3个方面进行综述,以期为蛋氨酸(methionine,Met)介导的反刍动物围产期营养调控研究与应用提供理论依据。

1 RPM营养调控作用

1.1 蛋氨酸的结构与功能
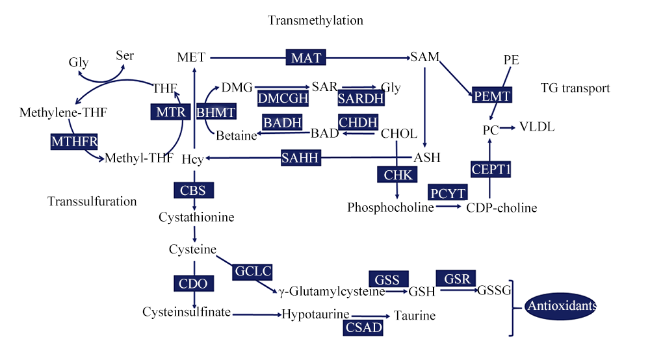
蛋氨酸相对分子质量为149.21,分子式为C5H11O2NS,分子中同时含有羧基、甲硫基和氨基,是必需氨基酸中唯一含有硫的氨基酸。蛋氨酸通过甲基、硫基循环合成胆碱、谷胱甘肽、胱氨酸、极低密度脂蛋白等产物,参与转硫氢基反应、转甲基反应、抗氧化和脂质代谢等过程(图1)[10]。蛋氨酸是反刍动物的第一或第二限制性氨基酸,也是维持反刍动物生长发育和各项生理活动的必需氨基酸。蛋氨酸参与机体蛋白质合成,在反刍动物泌乳期间,可作为底物和调控因子,通过分子信号通路促进乳腺蛋白质的合成[11];蛋氨酸还作为重要的甲基供体,在DNA甲基化[12]、肝脏一碳单位循环及脂质代谢[13]、炎症及氧化还原反应起到重要的调控作用[14],此外,蛋氨酸还促进畜禽生长[15]和繁殖性能[16],改善屠宰性能[17],促进绒毛的生长[18-19]
图1 蛋氨酸硫基与甲基循环过程

Transsulfuration:转硫基反应;Transmethylation:转甲基反应;Antioxidants:抗氧化剂;TG transport:甘油三酯转移;Betaine:甜菜碱;BAD:甜菜碱醛 betaine aldehyde;BADH:甜菜碱醛脱氢酶 betaine aldehyde dehydrogenase;BHMT:甜菜碱同型半胱氨酸甲基转移酶 betaine homocysteine methyltransferase;CBS:胱硫醚β胱合酶 cystathionine β-synthase;CDO:半胱氨酸双加氧酶 cysteine dioxygenase;CEPT1:胆碱/乙醇胺磷酸转移酶1 choline/ethanolamine phosphotransferase 1;CHDH:胆碱脱氢酶 choline dehydrogenase;CHK:胆碱激酶 choline kinase;Phosphocholine:磷酸胆碱;CHOL:胆碱 choline;CDP-choline:胞苷二磷酸胆碱 cytidine diphosphate choline;PC:磷脂酰胆碱 phosphatidylcholine;PCYT:磷酸胞苷酰转移酶 phosphate cytidylyltransferase;PE:磷脂酰乙醇胺 phosphatidylethanolamine;PEMT:磷脂酰乙醇胺甲基转移酶 phosphatidylethanolamine methyltransferase;CSAD:半胱氨酸亚磺酸脱羧酶 cysteine sulfinic acid decarboxylase;DMG:二甲基甘氨酸 dimethylglycine;DMGDH:二甲基甘氨酸脱氢酶 dimethylglycine dehydrogenase;GCLC:谷氨酸-半胱氨酸连接酶催化亚基 glutamate-cysteine ligase catalytic subunit;GSH:还原型谷胱甘肽 reduced glutathione;GSR:谷胱甘肽还原酶 glutathione reductase;GSS:谷胱甘肽合酶 glutathione synthase;GSSG:谷胱甘肽二硫化物 glutathione disulfide;Cystathionine:胱硫醚;Cysteine:半胱氨酸;Cysteinsulfinate:半胱氨酸亚磺酸盐;Hypotaurine:亚牛磺酸;Taurine:牛磺酸;γ-Glutamylcysteine:γ-谷氨酰半胱氨酸;Hcy:同型半胱氨酸 homocysteine;MAT:甲硫氨酸腺苷转移酶 methionine adenosyltransferase;MTHFR:亚甲基四氢叶酸还原酶 methylenetetrahydrofolate reductase;MTR:5-甲基四氢叶酸-同型半胱氨酸甲基转移酶 5-methyltetrahydrofolate-homocysteine methyltransferase;SAM:S-腺苷同型半胱氨酸 S-adenosylhomocysteine;SAHH:S-腺苷高半胱氨酸水解酶 S-adenosylhomocysteine hydrolase;SAM:S-腺苷甲硫氨酸 S-adenosylmethionine;SAR:肌氨酸 sarcosine;SARDH:肌氨酸脱氢酶 sarcosine dehydrogenase;THF:四氢叶酸 tetrahydrofolate。

Fig.1 Sulfur and methyl cycle process of methionine[10]

1.2 RPM的消化吸收特性

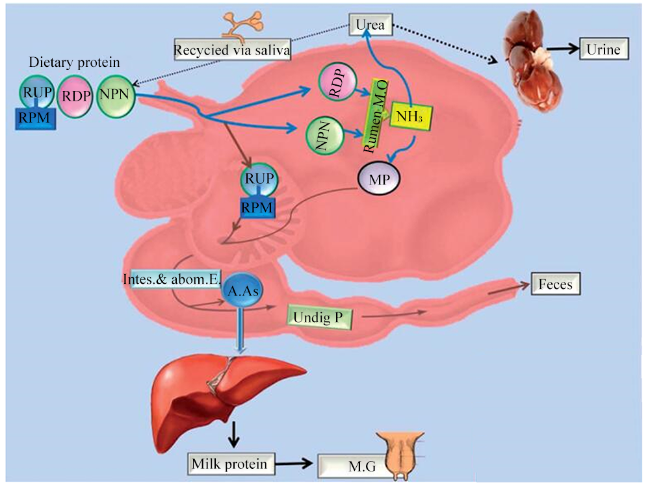
反刍动物可消化的蛋白质有2种:一种是瘤胃可降解蛋白质,被瘤胃微生物降解;另一种是瘤胃保护性蛋白质,它能保护蛋白质免受瘤胃微生物降解,而产生额外的氨基酸传递到小肠被吸收。RPM又称为瘤胃保护性蛋氨酸,就是运用过瘤胃技术,将蛋氨酸以某种方式修饰或保护起来,避免被瘤胃微生物分解,从而通过瘤胃被小肠吸收利用,在肝脏中分解代谢,并参与乳蛋白合成等生理过程(图2)[20]。近年来,围产期反刍动物补饲RPM对母体和后代生理状态、经济性状及相关调控机理研究逐渐成为研究热点,这对于实施围产期反刍动物精准营养调控和幼龄反刍动物的科学培育有重要意义。
图2 RPM的消化吸收特性

Dietary protein 饲粮蛋白质;RUP:瘤胃不可降解蛋白 rumen undegradable protein;RDP:瘤胃可降解蛋白 rumen degradable protein;NPN:非蛋白氮 non protein nitrogen;Recycied via saliva 通过唾液循环;Urea:尿素;Urine:尿;Rumen M.O:瘤胃微生物 rumen microorganism;MP:微生物蛋白质 microbial protein;NH3:氨气 ammonia;A.As:氨基酸 amino acids;Milk protein:乳蛋白;M.G:乳腺 mammary gland;Undig P:未消化蛋白质 undigested proteins;Feces:粪便。

Fig.2 Digestion and absorption characteristics of RPM[20]

1.3 RPM在反刍动物围产期的应用

围产期是反刍动物生产周期中最为关键的时期,分娩前后增加的营养需求、维持胎儿的生长、产后泌乳启动,加上自愿采食量的逐渐减少,对围产期反刍动物母体造成巨大的代谢压力,需要大量酶和活性物质的参与[21]。在围产期反刍动物的营养管理过程中,饲粮中添加过RPM可提高小肠氨基酸吸收率,为乳腺发育、泌乳启动、母体健康等做好蛋白质储备[10]。目前,RPM调控围产期反刍动物营养代谢和机体健康的研究主要有以下3个方面:1)RPM缓解围产期反刍动物的能量负平衡状态,促进甘油三酯转运,降低肝脏脂质沉积,增强糖异生过程,改善肝脏功能[2,22];2)RPM显著提高围产期奶牛[4,23-24]和母羊[3]的采食量、饲料转化效率、产奶量、乳脂率和乳蛋白含量,减少机体蛋白质动员,促进蛋白质平衡,提高产后泌乳性能;提高初乳中免疫和促生长因子含量,改善初乳品质[25]。但也有研究发现,补充RPM对奶牛[26-27]或奶山羊[28]的泌乳性能无明显影响,甚至有负面作用[29]。这可能与奶牛的泌乳阶段、饲粮组成(其他氨基酸的限制程度,尤其是赖氨酸)、不同RPM产品、试验设计[30]、饲粮本身的蛋氨酸含量[31]、个体差异[32]等因素相关。3)RPM增强围产期奶牛嗜中性粒细胞和单核细胞的吞噬能力,增加中性粒细胞的吞噬作用[33],下调促炎信号传导基因的表达[34],改善围产期奶牛和绵羊抗氧化状态[3,35],增强谷胱甘肽代谢[14],提高机体的抗氧化能力[36],促进围产期反刍动物的肝脏和机体健康。对围产期奶牛研究发现,RPM添加量为10~20 g/d(以蛋氨酸计)时,可以显著提高乳脂率,增加产奶量,提高生产性能[2]。对围产期母羊的研究发现,RPM添加量为2.5~5.0 g/d时,可提高其产奶量、乳蛋白含量、活体重、平均日增重和体增重,降低尿氮排出量、尿中尿素氮含量及其占食入氮比值,提高哺乳母羊整体生产性能[37]

2 围产期补饲RPM对幼龄反刍动物生长发育的影响

围产期反刍动物母体补饲RPM能够提高幼龄反刍动物的初生重、存活率,提升免疫机能,改善生产性能。

2.1 胎儿存活与宫内生长调控

Toledo等[38]发现围产期奶牛的子宫和胚胎液中富含蛋氨酸,表明蛋氨酸对胚胎正常生长和存活具有重要调控作用。子宫内蛋氨酸浓度的升高在正常胚胎生长和存活中发挥重要作用,对围产期奶牛饲喂RPM后血浆蛋氨酸浓度增加,促使乳中乳蛋白含量增加,改善经产奶牛的胚胎大小和妊娠维持。Ayyat等[37]报道进一步指出,RPM在正常胚胎生长和存活中发挥重要作用,即子宫腔内必需氨基酸浓度的增加可以通过血管壁和子宫内膜组织运输,支持和滋养胎儿的发育,与Groebner等[39]观点一致。因此,母体RPM的供应能够提高胚胎的存活率,促进胎儿的生长和发育。

2.2 幼龄反刍动物的免疫力

Moradi等[8]研究显示,在妊娠后期增加绵羊母体RPM和赖氨酸的供应,羔羊的血浆免疫球蛋白G含量(出生第15天和第30天)和牛奶摄入量(从出生第2周开始)显著升高。同样地,妊娠后期增强母牛RPM的供应会维持母体内蛋氨酸的稳态,促进牛磺酸合成,调控细胞黏附和趋化性、氧化应激、Toll样受体信号转导等促炎及宿主防御等相关mRNA[如诱导型一氧化氮合酶2(nitric oxide synthase 2,NOS2)和红细胞衍生核因子2样蛋白2(nuclear factor erythroid-derived 2-like 2,NFE2L2)基因的表达上调,半胱氨酸蛋白酶8(caspase 8,CASP8)、髓过氧化物酶(myeloperoxidase,MPO)、肿瘤坏死因子(tumor necrosis factor,TNF)基因的表达下调],显著上调影响细胞分化和炎症功能的mirRNA(如miR125b、miR146a、miR155等)的表达,进而引起犊牛血液多形核白细胞炎症功能的变化[40-41]。另有研究发现,在母体中补充RPM、叶酸和钴时,还会对犊牛体内一些血浆标志物(如血浆结合珠蛋白含量下降)以及炎症反应其他相关因子[如白细胞介素-1β(interleukin-1β,IL-1β)、白细胞介素-10(interleukin-10,IL-10)、TNF、白细胞介素-1受体关联激酶1(interleukin-1 receptor associated kinase 1,IRAK1)、CXC趋化因子受体1(C-X-C motif chemokine receptor 1,CXCR1)下调]产生抑制效应[42],从而影响其幼畜免疫系统功能的调控。

2.3 围产期补饲RPM对幼龄反刍动物生产性能的影响

2.3.1 生长性能

研究显示,哺乳母羊饲喂低蛋白质饲粮时补饲RPM,羔羊的体重增长了10%[43],羔羊的增重和生长速率显著提高[9,44],增加了氮平衡[45]。围产期母体补饲RPM,犊牛[5,46]和羔羊[3]的平均日增重显著提高,犊牛具有更高的饲料转化率,但对断奶体重无显著影响[47]。但也有研究发现,妊娠后期补充RPM对羔羊[48-49]或犊牛[50]的初生体重无显著影响,其对后代出生体重增加的影响还需要进一步研究。

2.3.2 屠宰性能

Liu等[51]研究显示,围产期母羊补饲0.06%的RPM,其羔羊具有更高的体脂肪以及更低的滴水损失,肉质得以改善。同时,Zhang等[6]在围产期母羊的饲粮中添加0.06%的RPM,羔羊具有最佳的屠宰率、净肉重以及肌内粗蛋白质和粗脂肪含量,提高了饲料中蛋白质利用效率,改善了羔羊的生长性能和肉质。

2.3.3 绒毛品质

研究发现,胎儿期的毛囊发育所需蛋氨酸能通过母体获得。Knipfel等[52]给母羊注射S35-蛋氨酸,发现蛋氨酸在胎儿期内毛囊发育过程中起到关键促进作用。Souri等[53]在离体培养毛囊时利用蛋氨酸同位素标记手段,发现蛋氨酸存在转硫基作用并合成半胱氨酸/胱氨酸,使生长期次级毛囊的生长达到最高速率。高晔等[54]研究发现,陕北白绒山羊妊娠期母羊饲粮中添加蛋氨酸,可以促进母羊与胎儿期羔羊的绒毛生长,还可以提高羔羊的初生重。

3 围产期补饲RPM对幼畜生长发育的调控机制

随着对反刍动物围产期营养生理学和表观遗传学研究的深入,发现RPM可提高母体血液甲基供体含量,影响一碳单位循环和蛋氨酸代谢,影响瘤胃微生物组成,调控分子信号通路,维持其泌乳性能和肝脏健康,进而促进后代的生长发育过程。

3.1 RPM改善产后泌乳性能调控幼龄反刍动物生长发育机制

妊娠后期母体的营养状况对胎儿发育有重要作用,对幼畜来说,母乳是其在能采食饲料之前唯一的营养物质和免疫球蛋白来源,是其出生到断奶最重要的营养物质来源,也是其出生后一定时期内生长发育都不可或缺的食物来源[55]。幼畜的生长发育与摄入母体的泌乳量及乳成分有直接关系。Titi等[49]用RPM补饲围产期奶牛,能够增加牛奶中乳蛋白含量,导致C4∶0~C12∶0脂肪酸的比例降低和C16∶0~C18∶3脂肪酸的比例增加。Sevi等[56]发现补充RPM导致母羊乳脂C16∶0~18∶3(主要是棕榈酸和硬脂酸)脂肪酸的比例增加,而C4∶0~12∶0脂肪酸的比例减少,不饱和饱和脂肪酸的比例也有适度的增加。Tsiplakou等[3]给围产期母羊补饲2.5 g/kg RPM,显著增加了母羊的乳脂和总固形物含量,羔羊的生长速度显著增加。Toledo等[57]进一步研究发现,RPM可通过增加血浆蛋氨酸浓度,增加乳蛋白的产量。给围产期奶牛补饲RPM,奶牛干物质采食量、初乳质量及能量校正乳、乳脂、蛋白质和乳糖含量显著升高,犊牛血清总蛋白和免疫球蛋白含量显著升高,新生犊牛被动免疫建立占比增加,平均日增重极显著增加[58]。因此,围产期反刍动物补充RPM能够改善产后泌乳性能,影响母乳营养成分,增加乳蛋白含量,影响脂肪酸比例,促进幼龄反刍动物建立被动免疫功能,增加平均日增重,促进其生长发育。

3.2 RPM介导的一碳循环调控幼龄反刍动物生长发育机制

对围产期母牛补饲RPM还能够提高血浆其他氨基酸的利用率,如谷氨酰胺、甘氨酸、丝氨酸、蛋氨酸等[59],血液蛋氨酸含量的升高,还能通过一碳循环合成胆碱、谷胱甘肽和牛磺酸等产物,对反刍动物适应代谢、应激等挑战起到重要调控作用[2]。在整个妊娠过程中,母体通过血液循环经胎盘传递为子代提供营养物质,胎盘是母体与胎儿间的重要免疫屏障,是激素获得和多肽吸收的重要途径[60]。胚胎发育期营养水平可能导致骨骼结构、生理功能和代谢能力发生永久性的变化[23]。研究显示,围产期奶牛补充RPM能够增加胎盘组织营养物质转运蛋白的丰度,提高胎儿对营养物质的利用效率,促进子宫以及幼龄反刍动物断奶前和断奶后早期的生长[6]。Groebner等[39]研究发现,子宫腔内必需氨基酸的增加通过血管壁和子宫内膜组织运输,支持和滋养胎儿的发育,这可能导致羔羊出生体重增加。RPM补充还改变了产后奶牛血浆氨基酸浓度,并增加了中性粒细胞浸润,提高子宫免疫力[61]。Hammon等[62]研究发现,围产期奶牛补充RPM增强了犊牛肝脏糖异生、脂肪酸氧化以及胰岛素敏感性,这对于出生后的犊牛的小腿发育是有利的。Alharthi等[5]研究发现,妊娠晚期奶牛供应RPM能够维持小牛蛋氨酸稳态,促进磷脂酰胆碱和牛磺酸合成、DNA甲基化和能量代谢,进而调控小牛的肝脏代谢。犊牛肝脏经历更快的糖异生和脂肪酸氧化成熟,有利于其适应宫外的代谢需求[63]。对妊娠后期母羊补充RPM,也能够增加羔羊肝脏能量代谢,调控其炎症反应[64]
因此,围产期反刍动物补饲RPM,可能通过蛋氨酸一碳循环,增加母体营养或活性物质(胆碱、谷胱甘肽和牛磺酸等),增强胎盘对营养物质的利用效率,促进胎儿的发育,增强后代糖异生、脂肪酸氧化成熟、胰岛素的敏感性,调控后代的肝脏代谢、免疫反应,使幼龄反刍动物更快的适应宫外环境,提高幼龄反刍动物的生长性能和免疫力。

3.3 RPM影响DNA或组蛋白甲基化调控幼龄反刍动物生长发育机制

围产期反刍动物补饲RPM,经小肠消化、吸收进入体内后转化为S-腺苷甲硫氨酸,提供游离甲基,引起肝脏及其他器官关键基因启动子区的甲基化,调控基因和调控因子的表达及相关代谢,这种效应可遗传给后代[65]。S-腺苷甲硫氨酸是DNA和组蛋白转甲基化的主要甲基供体,参与甲基循环。研究显示,母体营养会影响DNA和组蛋白甲基化的表观遗传机制[66],导致胚胎的DNA和/或组蛋白甲基化发生变化,间接影响胎儿发育和后代生理[67]
围产期奶牛补饲RPM,甲基供体的提供改变了新生犊牛肝脏一碳单位循环、蛋氨酸代谢和转硫反应等过程相关基因的表达,不同程度促进血多形核白细胞同型半胱氨酸的合成,减少活性氧积累,提高抗氧化能力和免疫功能[68],调控细胞黏附和趋化性、氧化应激、Toll样受体信号转导和蛋氨酸代谢相关的mRNA和miRNA表达的变化,提高免疫力[1];调控转录因子的表达,在母体蛋氨酸诱导的甲基化效应中发挥核心作用,维持蛋氨酸稳态、促进磷脂酰胆碱和牛磺酸合成、引起DNA甲基化和能量代谢变化,促进后代肝脏代谢[5];增加过氧化物酶体增殖物激活受体ɑ(peroxisome proliferator activated receptor alpha,PPARa)启动子区域甲基化;表明补充蛋氨酸可能通过合成S-腺苷甲硫氨酸激活肝脏PPARa调节的信号通路,改善脂质代谢和免疫功能[22]。研究还发现,对围产期母羊补饲2 g瘤胃保护蛋氨酸、300 mg叶酸、1.2 g硫、0.7 mg钴,不仅能够改善羔羊的胰岛素敏感性,还能够增加胰岛素的代谢清除率和β细胞的数量,且甲基供体补充的效果至少持续到羔羊出生后的第3周[69]。同时,在妊娠后期母羊补饲n-3多不饱和脂肪酸和蛋氨酸,还可以增加胎儿肝脏整体DNA甲基化,降低促炎细胞因子和脂肪生成基因mRNA的相对表达量,上调DNA-甲基转移酶的表达[70]。母羊补饲锌和蛋氨酸时,能够提升羔羊的肝脏器官指数,并通过血锌调节的锌指蛋白Sp3间接调控羔羊肝脏和脾脏中相关基因甲基化的表达,从而增强了后代免疫系统的发育和功能[71]
因此,围产期反刍动物补饲RPM能够提供游离甲基,胚胎通过胎盘摄取母体的甲基供体,影响后代DNA和组蛋白甲基化,调控相应基因的表达,促进幼龄反刍动物肝脏代谢,增强免疫系统功能,提高免疫力,促进幼龄反刍动物的生长发育。

3.4 RPM介导微生物组成与功能调控幼龄反刍动物生长发育

在围产期反刍动物中,奶牛饲粮从产犊前的高草料转变为产后高蛋白质饲粮,为瘤胃微生物群落提供更易获取的能量,微生物组成发生变化,有利于产生更多的挥发性脂肪酸和微生物蛋白质,为机体和乳汁合成提供能量和氨基酸来源[72-73]。瘤胃菌群与牛奶产量、乳脂率和乳蛋白率显著相关[74],牛奶产量和组成与瘤胃微生物多样性密切相关,且厚壁菌门与拟杆菌门之比和乳脂产量之间存在很强的相关性[74]。Abdelmegeid等[75]研究围产期奶牛补饲RPM对瘤胃微生物的影响,结果显示,当组间干物质采食量相似时,RPM可显著增加琥珀酸纤维杆菌、解淀粉单胞菌和解糖解糖杆菌的相对丰度。同时,Vailati-Riboni等[76]在泌乳中期奶牛饲粮中补饲RPM,发现瘤胃微生物组成发生了显著变化,丰度高的醋酸杆菌属(Acetobacter)、未鉴定_f_毛螺菌科(unclassified_f_Lachnospiraceae)和酵母菌有助于改善乳脂,且高温放线菌属(Thermoactinomyces)、无甾醇原体属菌(Asteroleplasma)和Saccharofermentan的丰度和牛奶中较高的α-酮戊二酸含量呈正相关。因此,RPM可能介导围产期反刍动物的瘤胃微生物,进而促进乳产量、乳蛋白和乳脂率,影响后代的生长发育。

3.5 RPM介导哺乳动物雷帕霉素靶点(mammalian target of rapamycin, mTOR)信号通路调控幼龄反刍动物生长发育

mTOR是高度保守的丝氨酸/苏氨酸蛋白激酶,在翻译水平通过影响mRNA与43S起始复合物的结合以及真核翻译起始因子4E结合蛋白1(eukaryotic translation initiation factor 4E-binding protein 1,4EBP1)和核糖体蛋白S6激酶1(ribosomal protein S6 kinase 1,S6K1)的磷酸化,调控乳蛋白的合成[77-78]。Liu等[79]对哺乳母羊提供蛋氨酸,结果发现mTORC1途径和全身氨基酸分解代谢是乳蛋白合成变化的驱动因素。进一步对RPM的诸多研究显示,对泌乳奶牛补饲RPM,其通过刺激mTOR信号通路增加乳蛋白产量,这种产量变化是由母体增加的干物质采食量所导致[80]。在妊娠后期增加RPM供应会导致母体干物质采食量、血浆蛋氨酸和胰岛素浓度增加,这些变化很可能会通过胎盘葡萄糖-氨基酸转运蛋白和mTOR信号通路蛋白的上调,刺激营养物质从母体向胎儿循环,从而在妊娠后期促进胎儿的生长[81-82]。Xu等[83]对妊娠后期奶牛补饲RPM,发现新生小牛肝脏mTOR信号通路的蛋白磷酸化水平显著升高,说明在妊娠晚期蛋氨酸的供应可能通过激活mTOR信号通路磷酸化调控犊牛肝脏代谢。因此,RPM不仅可以增加围产期反刍动物的干物质采食量,增加血浆营养成分,还能够通过mTOR信号通路刺激胎儿营养物质的转运效率,促进母体乳蛋白含量的增加,调控后代肝脏代谢,影响其生长发育过程。

4 小结

围产期反刍动物母体的营养状况对胎儿发育和幼龄后代的生产性能、炎症反应和氧化应激、产毛及屠宰性能等都有十分关键的调控作用。RPM主要通过一碳循环及蛋氨酸代谢、甲基循环、微生物及mTOR信号通路,增加围产期母体营养、活性物质和游离甲基,增强胚胎通过胎盘摄取母体物质的利用效率,促进胎儿的发育,影响后代DNA和组蛋白甲基化来调控相应基因的表达,影响微生物组成与功能,增强其糖异生、促进脂肪酸氧化成熟、改善胰岛素敏感性,促进幼龄反刍动物肝脏代谢和免疫系统发育,使幼龄反刍动物更快地适应宫外环境,提高生产性能和免疫力。未来研究重点关注以下3点:1)围产期反刍动物母体补饲RPM时,应以饲粮代谢蛋白质、氮和氨基酸平衡为基础,规范添加量和添加标准,合理与其他氨基酸或微量元素组合添加,如赖氨酸、不饱和脂肪酸、锌、钴等,以达到特定的研究目的。2)探究围产期反刍动物母体蛋氨酸供应对后代生长发育调控的时间限制,合理安排围产期反刍动物的营养管理方案。3)围产期反刍动物母体蛋氨酸供应对后代生长发育的调控机制研究还需进一步开展,明确其对后代生产性能、免疫及屠宰性能等存在的调控作用,揭示更多蛋氨酸代谢和一碳循环的生理机制,乳脂、乳蛋白、肝脏代谢等的调控信号通路,瘤胃和肠道核心微生物等,为幼龄反刍动物的培育提供更多理论支撑。
[1]
ABUELO A. Symposium review:late-gestation maternal factors affecting the health and development of dairy calves[J]. Journal of Dairy Science, 2020, 103(4):3882-3893.

DOI

[2]
孙菲菲. 胆碱和蛋氨酸对奶牛围产期营养平衡和机体健康的影响及机制[D]. 博士学位论文. 杨凌: 西北农林科技大学, 2017.

SUN F F. Choline and methionine regulate nutrient balance and health of transition dairy cows:responses and potential mechnisms[D]. Ph.D.Thesis. Yangling: Northwest A&F University, 2017. (in Chinese)

[3]
TSIPLAKOU E, MAVROMMATIS A, KALOGEROPOULOS T, et al. The effect of dietary supplementation with rumen-protected methionine alone or in combination with rumen-protected choline and betaine on sheep milk and antioxidant capacity[J]. Journal of Animal Physiology and Animal Nutrition, 2017, 101(5):1004-1013.

DOI PMID

[4]
ELSAADAWY S A, WU Z H, WANG H, et al. Supplementing ruminally protected lysine,methionine,or combination improved milk production in transition dairy cows[J]. Frontiers in Veterinary Science, 2022, 9:780637.

DOI

[5]
ALHARTHI A S, BATISTEL F, ABDELMEGEID M K, et al. Maternal supply of methionine during late-pregnancy enhances rate of Holstein calf development in utero and postnatal growth to a greater extent than colostrum source[J]. Journal of Animal Science and Biotechnology, 2018, 9(1):83.

DOI

[6]
ZHANG J H, LI H H, ZHANG G J, et al. Supplementation of guanidinoacetic acid and rumen-protected methionine increased growth performance and meat quality of Tan lambs[J]. Animal Bioscience, 2022, 35(10):1556-1565.

DOI

[7]
ELOLIMY A, ALHARTHI A, ZEINELDIN M, et al. Supply of methionine during late-pregnancy alters fecal microbiota and metabolome in neonatal dairy calves without changes in daily feed intake[J]. Frontiers in Microbiology, 2019, 10:2159.

DOI PMID

[8]
MORADI M, CHASHNIDEL Y, TEIMOURI YANSARI A, et al. Moderate overfeeding of different sources of metabolizable energy and protein.Ⅱ:Effects on inflammatory status of sheep in late pregnancy and growth trajectory of the offspring[J]. Theriogenology, 2021, 176:115-121.

DOI

[9]
TITI H H, ALNIMER M A, ABEDAL-MAJED M A. Effect of supplemental rumen-protected methionine on reproduction and production of Awassi ewes[J]. Italian Journal of Animal Science, 2022, 21(1):624-633.

DOI

[10]
ZHOU Z, GARROW T A, DONG X W, et al. Hepatic activity and transcription of betaine-homocysteine methyltransferase,methionine synthase,and cystathionine synthase in periparturient dairy cows are altered to different extents by supply of methionine and choline[J]. The Journal of Nutrition, 2017, 147(1):11-19.

DOI

[11]
QI H, MENG C Y, JIN X, et al. Methionine promotes milk protein and fat synthesis and cell proliferation via the SNAT2-PI3K signaling pathway in bovine mammary epithelial cells[J]. Journal of Agricultural and Food Chemistry, 2018, 66(42):11027-11033.

DOI PMID

[12]
BATISTEL F, ALHARTHI A S, YAMBAO R R C, et al. Methionine supply during late-gestation triggers offspring sex-specific divergent changes in metabolic and epigenetic signatures in bovine placenta[J]. The Journal of Nutrition, 2019, 149(1):6-17.

DOI

[13]
LIANG Y, BATISTEL F, PARYS C, et al. Methionine supply during the periparturient period enhances insulin signaling,amino acid transporters,and mechanistic target of rapamycin pathway proteins in adipose tissue of Holstein cows[J]. Journal of Dairy Science, 2019, 102(5):4403-4414.

DOI

[14]
LIANG Y, BATISTEL F, PARYS C, et al. Glutathione metabolism and nuclear factor erythroid 2-like 2 (NFE2L2)-related proteins in adipose tissue are altered by supply of ethyl-cellulose rumen-protected methionine in peripartal Holstein cows[J]. Journal of Dairy Science, 2019, 102(6):5530-5541.

DOI PMID

[15]
ZHAI W, ARAUJO L F, BURGESS S C, et al. Protein expression in pectoral skeletal muscle of chickens as influenced by dietary methionine[J]. Poultry Science, 2012, 91(10):2548-2555.

PMID

[16]
田孟芳, 甘富斌, 赵彦玲. 蛋氨酸对畜禽繁殖性能的影响[J]. 中国畜禽种业, 2019, 15(3):80.

TIAN M F, GAN F B, ZHAO Y L. Effects of methionine on reproductive performance of livestock and poultry[J]. The Chinese Livestock and Poultry Breeding, 2019, 15(3):80. (in Chinese)

[17]
WEN C, WU P, CHEN Y P, et al. Methionine improves the performance and breast muscle growth of broilers with lower hatching weight by altering the expression of genes associated with the insulin-like growth factor-I signaling pathway[J]. British Journal of Nutrition, 2014, 111(2):201-206.

DOI

[18]
WYROSTEK A, KINAL S, PATKOWSKA-SOKOŁA B, et al. The influence of zinc-methionine bioplex supplementation to pregnant and lactating sheep on selected wool parameters[J]. Archives Animal Breeding, 2019, 62(1):99-105.

DOI PMID

[19]
王文楠, 孙亚波, 刘海英, 等. 蛋氨酸对动物生长发育及毛发生长调控作用的研究进展[J]. 中国饲料, 2019(5):4-7.

WANG W N, SUN Y B, LIU H Y, et al. Research progress of methionine on animal growth and regulation of hair growth[J]. China Feed, 2019(5):4-7. (in Chinese)

[20]
KAMALAK A, CANBOLAT Ö, GÜRBÜZ Y, et al. Protected protein and amino acids in ruminant nutrition[J]. KSU.Journal of Science and Engineering, 2005, 8(2):84-88.

[21]
JI P, DANN H M. Negative protein balance:implications for fresh and transition cows[J]. Journal of Dairy Research, 2002, 11(2):2-6.

[22]
OSORIO J S, JACOMETO C B, ZHOU Z, et al. Hepatic global DNA and peroxisome proliferator-activated receptor alpha promoter methylation are altered in peripartal dairy cows fed rumen-protected methionine[J]. Journal of Dairy Science, 2016, 99(1):234-244.

DOI PMID

[23]
TOLEDO M Z, STANGAFERRO M L, GENNARI R S, et al. Effects of feeding rumen-protected methionine pre- and postpartum in multiparous Holstein cows:lactation performance and plasma amino acid concentrations[J]. Journal of Dairy Science, 2021, 104(7):7583-7603.

DOI

[24]
JUNIOR V C, LOPES F, SCHWAB C G, et al. Effects of rumen-protected methionine supplementation on the performance of high production dairy cows in the tropics[J]. PLoS One, 2021, 16(4):e0243953.

DOI

[25]
王瀚. 围产前期日粮添加过瘤胃蛋氨酸对初乳和犊牛生长的影响[D]. 硕士学位论文. 秦皇岛: 河北科技师范学院, 2021.

WANG H. Effects of rumen-protected methionine supplements in transition diets of dairy cows on the colostrum and growth performance of calves[D]. Master’s Thesis. Qinhuangdao: Hebei Normal University of Science & Technology, 2021. (in Chinese)

[26]
SOCHA M T, PUTNAM D E, GARTHWAITE B D, et al. Improving intestinal amino acid supply of pre- and postpartum dairy cows with rumen-protected methionine and lysine[J]. Journal of Dairy Science, 2005, 88(3):1113-1126.

PMID

[27]
DAVIDSON S, HOPKINS B A, ODLE J, et al. Supplementing limited methionine diets with rumen-protected methionine,betaine,and choline in early lactation Holstein cows[J]. Journal of Dairy Science, 2008, 91(4):1552-1559.

DOI

[28]
ALONSO-MÉLENDEZ E, MENDOZA G D, CASTREJÓN-PINEDA F A, et al. Milk production in dairy goats supplemented with different levels of ruminally protected methionine[J]. Journal of Dairy Research, 2016, 83(2):148-150.

DOI

[29]
BENEFIELD B C, PATTON R A, STEVENSON M J, et al. Evaluation of rumen-protected methionine sources and period length on performance of lactating dairy cows within Latin squares[J]. Journal of Dairy Science, 2009, 92(9):4448-4455.

DOI PMID

[30]
PATTON R A. Effect of rumen-protected methionine on feed intake,milk production,true milk protein concentration,and true milk protein yield,and the factors that influence these effects:a Meta-analysis[J]. Journal of Dairy Science, 2010, 93(5):2105-2118.

DOI

[31]
ZANTON G I, BOWMAN G R, VÁZQUEZ-AÑÓN M, et al. Meta-analysis of lactation performance in dairy cows receiving supplemental dietary methionine sources or postruminal infusion of methionine[J]. Journal of Dairy Science, 2014, 97(11):7085-7101.

DOI PMID

[32]
梁树林. 奶牛泌乳性能对过瘤胃蛋氨酸响应的个体差异及其成因探究[D]. 博士学位论文. 杭州: 浙江大学, 2021.

LIANG S L. Inter-individual variability and causality in the lactation performance in response to rumen-protected methionine in lactating dairy cows[D]. Ph.D.Thesis. Hangzhou: Zhejiang University, 2021. (in Chinese)

[33]
OSORIO J S, JI P, DRACKLEY J K, et al. Supplemental Smartamine M or MetaSmart during the transition period benefits postpartal cow performance and blood neutrophil function[J]. Journal of Dairy Science, 2013, 96(10):6248-6263.

DOI PMID

[34]
TSIPLAKOU E, MAVROMMATIS A, SKLIROS D, et al. The impact of rumen-protected amino acids on the expression of key- genes involved in the innate immunity of dairy sheep[J]. PLoS One, 2020, 15(5):e0233192.

DOI

[35]
ZHOU Z, VAILATI-RIBONI M, LUCHINI D N, et al. Methionine and choline supply during the periparturient period alter plasma amino acid and one-carbon metabolism profiles to various extents:potential role in hepatic metabolism and antioxidant status[J]. Nutrients, 2016, 9(1):10.

DOI

[36]
HAN L, BATISTEL F, MA Y, et al. Methionine supply alters mammary gland antioxidant gene networks via phosphorylation of nuclear factor erythroid 2-like 2 (NFE2L2) protein in dairy cows during the periparturient period[J]. Journal of Dairy Science, 2018, 101(9):8505-8512.

DOI PMID

[37]
AYYAT M S, AL-SAGHEER A, NORELDIN A E, et al. Beneficial effects of rumen-protected methionine on nitrogen-use efficiency,histological parameters,productivity and reproductive performance of ruminants[J]. Animal Biotechnology, 2021, 32(1):51-66.

DOI

[38]
TOLEDO M Z, BAEZ G M, GARCIA-GUERRA A, et al. Effect of feeding rumen-protected methionine on productive and reproductive performance of dairy cows[J]. PLoS One, 2017, 12(12):e0189117.

DOI

[39]
GROEBNER A E, RUBIO-ALIAGA I, SCHULKE K, et al. Increase of essential amino acids in the bovine uterine lumen during preimplantation development[J]. Reproduction, 2011, 141(5):685-695.

DOI PMID

[40]
ALHARTHI A S, COLEMAN D N, LIANG Y, et al. Hepatic 1-carbon metabolism enzyme activity,intermediate metabolites,and growth in neonatal Holstein dairy calves are altered by maternal supply of methionine during late pregnancy[J]. Journal of Dairy Science, 2019, 102(11):10291-10303.

DOI

[41]
JACOMETO C B, ALHARTHI A S, ZHOU Z, et al. Maternal supply of methionine during late pregnancy is associated with changes in immune function and abundance of microRNA and mRNA in Holstein calf polymorphonuclear leukocytes[J]. Journal of Dairy Science, 2018, 101(9):8146-8158.

DOI PMID

[42]
LOPES M G, ALHARTHI A S, LOPREIATO V, et al. Maternal supplementation with cobalt sources,folic acid,and rumen-protected methionine and its effects on molecular and functional correlates of the immune system in neonatal Holstein calves[J]. Journal of Dairy Science, 2021, 104(8):9340-9354.

DOI

[43]
LIU S M, LEI J, HANCOCK S, et al. Lamb survival,glutathione redox state and immune function of neonates and lambs from periparturient Merino ewes supplemented with rumen-protected methionine[J]. Archives of Animal Nutrition, 2016, 70(5):389-401.

DOI

[44]
AWAWDEH M S. Effects of supplemental lysine and methionine on performance of nursing Awassi ewes fed two levels of dietary protein[J]. Tropical Animal Health and Production, 2022, 54(1):61.

DOI PMID

[45]
LYNCH G P, ELSASSER T H, JACKSON C,Jr, et al. Nitrogen metabolism of lactating ewes fed rumen-protected methionine and lysine[J]. Journal of Dairy Science, 1991, 74(7):2268-2276.

PMID

[46]
WANG H, ELSAADAWY S A, WU Z H, et al. Maternal supply of ruminally-protected lysine and methionine during close-up period enhances immunity and growth rate of neonatal calves[J]. Frontiers in Veterinary Science, 2021, 8:780731.

DOI

[47]
SILVA G M, CHALK C D, RANCHES J, et al. Effect of rumen-protected methionine supplementation to beef cows during the periconception period on performance of cows,calves,and subsequent offspring[J]. Animal, 2021, 15(1):100055.

DOI

[48]
AL-QAISI M A, TITI H H. Effect of rumen-protected methionine on production and composition of early lactating Shami goats milk and growth performance of their kids[J]. Archives Animal Breeding, 2014, 57(1):1-11.

[49]
TITI H H. Effect of long-term rumen-protected methionine supplementation on performance of Shami goats and growth performance of their kids[J]. Animal Production Science, 2016, 57(8):1713-1718.

DOI

[50]
CLEMENTS A R, IRELAND F A, FREITAS T, et al. Effects of supplementing methionine hydroxy analog on beef cow performance,milk production,reproduction,and preweaning calf performance[J]. Journal of Animal Science, 2017, 95(12):5597-5605.

DOI

[51]
LIU H, YANG G, DEGEN A, et al. Effect of feed level and supplementary rumen protected lysine and methionine on growth performance,rumen fermentation,blood metabolites and nitrogen balance in growing Tan lambs fed low protein diets[J]. Animal Feed Science and Technology, 2021, 279:115024.

DOI

[52]
KNIPFEL J E, ELLIOT J I, WILLES R F. Distribution of methionine and its metabolites in the pregnant ewe and fetus following intravenous or abomasal injection of 35S-methionine into the ewe[J]. Canadian Journal of Animal Science, 1986, 66(4):959-973.

DOI

[53]
SOURI M, GALBRAITH H, SCAIFE J R. Conversion of methionine to cysteine by transulphuration in isolated anagen secondary hair follicles of the Angora goat[J]. Proceedings of the British Society of Animal Science, 1998, 1998:139.

DOI

[54]
高晔, 闫海龙, 闫玉清, 等. 妊娠期绒山羊母羊饲粮添加过瘤胃蛋氨酸对羔羊绒毛品质的影响[J]. 家畜生态学报, 2019, 40(8):37-41.

GAO Y, YAN H L, YAN Y Q, et al. Effect of rumen protected methionine on growth performance and fleece quality of pregnant and newborn cashmere goats[J]. Acta Ecologae Animalis Domastici, 2019, 40(8):37-41. (in Chinese)

[55]
陈杰. 家畜生理学[M]. 4版. 北京: 中国农业出版社, 2003.

CHEN J. Physiology of domestic animals[M]. 4th ed. Beijing: China Agriculture Press, 2003. (in Chinese)

[56]
SEVI A, ROTUNNO T, DI CATERINA R, et al. Rumen-protected methionine or lysine supplementation of Comisana ewes’ diets:effects on milk fatty acid composition[J]. Journal of Dairy Research, 1998, 65(3):413-422.

DOI

[57]
ELSAADAWY S A E. 围产期奶牛日粮添加过瘤胃保护赖氨酸和蛋氨酸对其生产性能及新生犊牛生长的影响[D]. 博士学位论文. 北京: 中国农业科学院, 2021.

ELSAADAWY S A E. Effect of dietary supplementing ruminally-protected lysine and methionine during transition on the performance of cows and calves[D]. Ph.D.Thesis. Beijing: Chinese Academy of Agricultural Sciences, 2021. (in Chinese)

[58]
WATERMAN R C, UJAZDOWSKI V L, PETERSEN M K. Effects of rumen-protected methionine on plasma amino acid concentrations during a period of weight loss for late gestating beef heifers[J]. Amino Acids, 2012, 43(5):2165-2177.

DOI PMID

[59]
GODFREY K, ROBINSON S, BARKER D J, et al. Maternal nutrition in early and late pregnancy in relation to placental and fetal growth[J]. BMJ, 1996, 312(7028):410-414.

PMID

[60]
WADHWA P D, BUSS C, ENTRINGER S, et al. Developmental origins of health and disease:brief history of the approach and current focus on epigenetic mechanisms[J]. Seminars in Reproductive Medicine, 2009, 27(5):358-368.

DOI

[61]
STELLA S L, VELASCO-ACOSTA D A, SKENANDORE C, et al. Improved uterine immune mediators in Holstein cows supplemented with rumen-protected methionine and discovery of neutrophil extracellular traps (NET)[J]. Theriogenology, 2018, 114:116-125.

DOI PMID

[62]
HAMMON H M, STEINHOFF-WAGNER J, SCHÖNHUSEN U, et al. Energy metabolism in the newborn farm animal with emphasis on the calf:endocrine changes and responses to milk-born and systemic hormones[J]. Domestic Animal Endocrinology, 2012, 43(2):171-185.

DOI

[63]
JACOMETO C B, ZHOU Z, LUCHINI D, et al. Maternal rumen-protected methionine supplementation and its effect on blood and liver biomarkers of energy metabolism,inflammation,and oxidative stress in neonatal Holstein calves[J]. Journal of Dairy Science, 2016, 99(8):6753-6763.

DOI

[64]
ROSA-VELAZQUEZ M, PINOS-RODRIGUEZ J M, PARKER A J, et al. Maternal supply of a source of omega-3 fatty acids and methionine during late gestation on the offspring’s growth,metabolism,carcass characteristic,and liver’s mRNA expression in sheep[J]. Journal of Animal Science, 2022, 100(4):skac032.

DOI

[65]
JACOMETO C B, ZHOU Z, LUCHINI D, et al. Maternal supplementation with rumen-protected methionine increases prepartal plasma methionine concentration and alters hepatic mRNA abundance of 1-carbon,methionine,and transsulfuration pathways in neonatal Holstein calves[J]. Journal of Dairy Science, 2017, 100(4):3209-3219.

DOI

[66]
MENTCH S J, LOCASALE J W. One-carbon metabolism and epigenetics:understanding the specificity[J]. Annals of the New York Academy of Sciences, 2016, 1363(1):91-98.

DOI

[67]
XU J, SINCLAIR K D. One-carbon metabolism and epigenetic regulation of embryo development[J]. Reproduction,Fertility,and Development, 2015, 27(4):667-676.

DOI

[68]
CHANDLER T L, WHITE H M. Choline and methionine differentially alter methyl carbon metabolism in bovine neonatal hepatocytes[J]. PLoS One, 2017, 12(2):e0171080.

DOI

[69]
SULAIMAN S A, DE BLASIO M J, HARLAND M L, et al. Maternal methyl donor and cofactor supplementation in late pregnancy increases β-cell numbers at 16 days of life in growth-restricted twin lambs[J]. American Journal of Physiology:Endocrinology and Metabolism, 2017, 313(4):E381-E390.

DOI

[70]
ROSA VELAZQUEZ M, BATISTEL F, PINOS RODRIGUEZ J M, et al. Effects of maternal dietary omega-3 polyunsaturated fatty acids and methionine during late gestation on fetal growth,DNA methylation,and mRNA relative expression of genes associated with the inflammatory response,lipid metabolism and DNA methylation in placenta and offspring’s liver in sheep[J]. Journal of Animal Science and Biotechnology, 2020, 11(1):111.

DOI

[71]
LI Q S, YAN Q X, ZHOU C S, et al. Effects of dietary zinc-methionine supplementation during pregnancy on the whole-genome methylation and related gene expression in the liver and spleen of growing goats:a short communication[J]. Biological Trace Element Research, 2021, 199(3):996-1001.

DOI

[72]
PITTA D W, KUMAR S, VECCHIARELLI B, et al. Temporal dynamics in the ruminal microbiome of dairy cows during the transition period[J]. Journal of Animal Science, 2014, 92(9):4014-4022.

DOI PMID

[73]
LIMA F S, OIKONOMOU G, LIMA S F, et al. Prepartum and postpartum rumen fluid microbiomes:characterization and correlation with production traits in dairy cows[J]. Applied and Environmental Microbiology, 2015, 81(4):1327-1337.

DOI

[74]
JAMI E, WHITE B A, MIZRAHI I. Potential role of the bovine rumen microbiome in modulating milk composition and feed efficiency[J]. PLoS One, 2014, 9(1):e85423.

DOI

[75]
ABDELMEGEID M K, ELOLIMY A A, ZHOU Z, et al. Rumen-protected methionine during the peripartal period in dairy cows and its effects on abundance of major species of ruminal bacteria[J]. Journal of Animal Science and Biotechnology, 2018, 9:17.

DOI PMID

[76]
VAILATI-RIBONI M, BATISTEL F, YAMBAO R R C S, et al. Hepatic cystathionine β-synthase activity is increased by greater postruminal supply of met during the periparturient period in dairy cows[J]. Current Developments in Nutrition, 2019, 3(12):nzz128.

[77]
DAI W T, WHITE R R, LIU J X, et al. Seryl-tRNA synthetase-mediated essential amino acids regulate β-casein synthesis via cell proliferation and mammalian target of rapamycin (mTOR) signaling pathway in bovine mammary epithelial cells[J]. Journal of Dairy Science, 2018, 101(11):10456-10468.

DOI PMID

[78]
DONG X, ZHOU Z, SAREMI B, et al. Varying the ratio of Lys:Met while maintaining the ratios of Thr:Phe,Lys:Thr,Lys:His,and Lys:Val alters mammary cellular metabolites, mammalian target of rapamycin signaling,and gene transcription[J]. Journal of Dairy Science, 2018, 101(2):1708-1718.

DOI

[79]
LIU W, XIA F, HANIGAN M D, et al. Short-term lactation and mammary metabolism responses in lactating goats to graded removal of methionine from an intravenously infused complete amino acid mixture[J]. Journal of Dairy Science, 2019, 102(5):4094-4104.

DOI PMID

[80]
ZHAO K, LIU W, LIN X Y, et al. Effects of rumen-protected methionine and other essential amino acid supplementation on milk and milk component yields in lactating Holstein cows[J]. Journal of Dairy Science, 2019, 102(9):7936-7947.

DOI PMID

[81]
SLETMOEN-OLSON K E, CATON J S, OLSON K C, et al. Undegraded intake protein supplementation:I.Effects on forage utilization and performance of periparturient beef cows fed low-quality hay[J]. Journal of Animal Science, 2000, 78(2):449-455.

DOI

[82]
BATISTEL F, ARROYO J M, BELLINGERI A, et al. Ethyl-cellulose rumen-protected methionine enhances performance during the periparturient period and early lactation in Holstein dairy cows[J]. Journal of Dairy Science, 2017, 100(9):7455-7467.

DOI PMID

[83]
XU T, ALHARTHI A S M, BATISTEL F, et al. Hepatic phosphorylation status of serine/threonine kinase 1,mammalian target of rapamycin signaling proteins,and growth rate in Holstein heifer calves in response to maternal supply of methionine[J]. Journal of Dairy Science, 2018, 101(9):8476-8491.

DOI

文章导航

/