研究论文

植物乳杆菌对小鼠体重、炎症反应及肠道健康的影响

  • 伊婷 , 1 ,
  • 乔家运 2 ,
  • 李玉鹏 3, 4, 5 ,
  • 李海花 , 1, *
展开
  • 1 天津农学院动物科学与动物医学学院,天津市农业动物繁育与健康养殖重点实验室,天津 300384
  • 2 天津师范大学生命科学学院,天津市动物多样性保护与利用重点实验室,天津 300387
  • 3 天津市农业科学院畜牧兽医研究所,天津 300381
  • 4 天津市畜禽分子育种与生物技术重点实验室,天津 300381
  • 5 天津市畜禽健康养殖工程技术中心,天津 300381
*李海花,副教授,硕士生导师,E-mail:

伊 婷(1999—),女,河南焦作人,硕士研究生,研究方向为动物性食品生产与安全。E-mail:

Copy editor: 菅景颖

收稿日期: 2022-09-06

  网络出版日期: 2023-04-12

基金资助

天津市自然科学基金(20JCZDJC00190)

天津市“131”创新型人才团队(20180338)

Effects of Lactobacillus plantarum on Body Weight, Inflammatory Response and Intestinal Health of Mice

  • YI Ting , 1 ,
  • QIAO Jiayun 2 ,
  • LI Yupeng 3, 4, 5 ,
  • LI Haihua , 1, *
Expand
  • 1 Tianjin Key Laboratory of Agricultural Animal Breeding and Healthy Husbandry, College of Animal Science and Veterinary Medicine, Tianjin Agricultural University, Tianjin 300384, China
  • 2 Tianjin Key Laboratory of Conservation and Utilization of Animal Diversity, College of Life Sciences, Tianjin Normal University, Tianjin 300387, China
  • 3 Institute of Animal Science and Veterinary, Tianjin Academy of Agricultural Sciences, Tianjin 300381, China
  • 4 Tianjin Key Laboratory of Animal Molecular Breeding and Biotechnology, Tianjin 300381, China
  • 5 Tianjin Engineering Research Center of Animal Healthy Farming, Tianjin 300381, China
*associate professor, E-mail:

Received date: 2022-09-06

  Online published: 2023-04-12

摘要

本试验旨在研究植物乳杆菌对小鼠体重、肠道形态、血清炎症因子、盲肠内容物短链脂肪酸(SCFAs)及肠道菌群的影响。试验选用20只8周龄雌性昆明小鼠,随机分为对照组和植物乳杆菌组,每组10只。植物乳杆菌组小鼠每日灌胃浓度为1×10⁹ CFU/mL的植物乳杆菌悬液,灌胃量为0.2 mL/只,对照组小鼠每日灌胃等量生理盐水。试验期为14 d。结果表明:1)与对照组相比,灌胃植物乳杆菌对小鼠体重、增重率没有显著影响(P>0.05)。2)与对照组相比,植物乳杆菌组小鼠空肠绒隐比显著上升(P<0.05)。3)与对照组相比,植物乳杆菌组盲肠内容物总SCFAs含量显著升高(P<0.05),而血清炎症因子[C-反应蛋白(CRP)、肿瘤坏死因子-α(TNF-α)、白细胞介素-8(IL-8)]含量无显著变化(P>0.05)。4)与对照组相比,植物乳杆菌组小鼠盲肠内容物中乳杆菌属的相对丰度极显著升高(P<0.01),有益菌相对丰度上升,同时潜在的致病菌相对丰度下降。综上所述,灌胃植物乳杆菌能够改善小鼠肠道形态,提高小肠吸收能力,提高优势菌属的相对丰度,有利于肠道健康。

本文引用格式

伊婷 , 乔家运 , 李玉鹏 , 李海花 . 植物乳杆菌对小鼠体重、炎症反应及肠道健康的影响[J]. 动物营养学报, 2023 , 35(4) : 2668 -2676 . DOI: 10.12418/CJAN2023.249

Abstract

This experiment was designed to investigate the effects of Lactobacillus plantarum on body weight, intestinal morphology, serum inflammatory factors, short-chain fatty acids (SCFAs) in cecal contents and intestinal flora of mice. Twenty 8-week-old female Kunming mice were randomly divided into control and Lactobacillus plantarum (LP) groups of 10 mice each. The mice in the LP group were gavaged with 1×10⁹ CFU/mL LP suspension on 2 mL per mouse daily for 14 days, while the mice in the control group were given the same amount of normal saline daily. The results showed as follows: 1) compared with the control group, gavage of LP had no significant effects on the body weight and weight gain rate of mice. 2) Compared with the control group, the ratio of villus height to crypt depth of jejunum in the LP group was significantly increased (P<0.05). 3) Compared with the control group, the total short chain fatty acids (SCFAs) content in the cecal content of mice in the LP group increased significantly (P<0.05), while the contents of serum inflammatory factors [C-reactive protein (CRP), tumor necrosis factor-α (TNF-α) and interleukin-8 (IL-8)] did not change significantly (P>0.05). 4) Compared with the control group, the relative abundance of Lactobacillus in the cecal contents of mice in the LP group was extremely significantly increased (P<0.01), and the relative abundance of beneficial bacteria increased, while the relative abundance of potentially pathogenic bacteria decreased. In conclusion, gavage of LP can improve the intestinal morphology of mice, enhance the absorption capacity of the small intestine, increase the relative abundance of the dominant genera, and benefit the intestinal health.

乳酸菌对机体有诸多有益作用,如调节肠道菌群环境、提高机体免疫能力、改善生长性能等[1]。植物乳杆菌(Lactobacillus plantarum,L. plantarum)是一种常见的乳酸菌,也是人体肠道微生物的重要成员。植物乳杆菌具有耐酸、抑菌、抗氧化、免疫调节以及缓解神经系统疾病[2-3]等作用。有研究表明,添加源自健康婴儿粪便的植物乳杆菌1258调节仔猪肠道固有免疫,可通过抑制Toll样受体(Toll-like receptor,TLR)介导的丝裂原活化蛋白激酶(mitogen activated protein kinase,MAPK)抵制产肠毒素型大肠杆菌K88(enterotoxigenic E. coil K88,ETEC K88)的攻击[4]。Schwarzer等[5]发现,在营养不良的情况下,从果蝇肠道中分离的菌种LP NIZO2877可调节小鼠幼体生长,肠道微生物群与促生长激素相互作用,进而改善慢性营养不良。Kuda等[6]通过对鱼的肠道菌群筛选分析,得到具有抗酸、抗胆汁和抗盐特性的乳酸菌菌群,其中4种鉴定为植物乳杆菌,它们具有较强的清除自由基能力。另外,有研究发现最初从人类唾液分离的植物乳杆菌WCFS1对抗炎活性相关基因有诱导作用,确定了与健康成人免疫耐受建立相关的黏膜基因表达模式和细胞通路[7]。本研究团队前期发现,从健康猪粪便中分离鉴定出的植物乳杆菌能有效抑制致病性大肠杆菌生长[8],能通过抑制p38 MAPK磷酸化和阻断核因子-κB(nuclear factor-κB,NF-κB)信号通路缓解产肠毒素型大肠杆菌引起的肠上皮细胞炎症反应,对肠道屏障功能有良好的改善效果[9]
小肠是体内微生物主要的存在部位,肠道形态能够直接反映肠道消化吸收的能力。肠道菌群是衡量机体健康状况的重要指标,菌群失调已被证实与多种疾病相关[10-11]。肠道菌群分解肠道内碳水化合物产生短链脂肪酸(short chain fatty acids,SCFAs),可为肠道微生物群提供营养[12]。然而,目前关于植物乳杆菌对动物肠道菌群调控方面的影响却鲜见报道。C-反应蛋白(C-reactive protein,CRP)是在组织受损时含量急剧上升的蛋白质[13],与肿瘤坏死因子-α(tumor necrosis factor-α,TNF-α)、白细胞介素-8(interleukin-8,IL-8)一起作为损伤标记物,提示炎症发生[14]。尽管已经明确植物乳杆菌能够抑制致病性大肠杆菌引起的肠上皮细胞炎症反应,具有多种益生作用,但是植物乳杆菌对动物机体单独作用时是否有致炎作用,以及对肠道健康的影响尚不十分清楚。本文以小鼠为试验动物,通过分析猪源植物乳杆菌对小鼠空肠结构、炎症相关指标、盲肠内容物SCFAs以及肠道菌群的影响,探究植物乳杆菌对小鼠炎症反应及肠道健康的影响,为植物乳杆菌在动物生产中的应用提供理论依据。

1 材料与方法

1.1 试验材料

试验用植物乳杆菌由天津农学院动物科学与动物医学学院实验室保存。将菌种进行增菌培养,计数后用生理盐水稀释至1×10⁹ CFU/mL用于后续试验。
试验动物为20只无特定病原体(SPF)级雄性昆明小鼠,约8周龄,体重21~23 g。自然光照下,小鼠饲养温度为22~25 ℃,采用自由饮水和采食的方式饲养。试验动物与饲粮均购自中国食品药品检定研究院。将20只小鼠随机分为2组,分别为对照组和植物乳杆菌组,每组10只,试验期为14 d。试验开始前3天进行预饲,试验开始后对照组小鼠每日灌胃生理盐水0.2 mL/只,植物乳杆菌组小鼠每日灌胃浓度为1×109 CFU/mL的植物乳杆菌悬液,灌胃量为0.2 mL/只。

1.2 样品采集

灌胃试验结束后,对照组和植物乳杆菌组分别随机取6只小鼠,摘除眼球取血至2 mL离心管中,3 000 r/min离心5 min分离血清,液氮速冻,置于-80 ℃密封保存用于血清学指标测定。
处死小鼠后,对照组和植物乳杆菌组各采集6只小鼠盲肠内容物于EP管中,置于-80 ℃密封保存用于SCFAs含量的测定和16S rDNA扩增子测序试验;将小肠的空肠部分浸于4%甲醛溶液内固定,用于制作组织切片。

1.3 测定指标与方法

1.3.1 体重的测定和增重率的计算

记录20只小鼠初始体重和终末体重,称重前小鼠禁食12 h;根据初始体重和终末体重计算增重率,计算公式如下:
增重率(%)=[(终末体重-初始体重)/初始体重]×100。

1.3.2 血清学指标及盲肠内容物SCFAs含量的测定

将血清样本取出于4 ℃解冻,采用酶联免疫吸附测定(ELISA)试剂盒(购于美国 BD 公司)测定血清中CRP、TNF-α以及IL-8的含量。将盲肠内容物从-80 ℃取出于4 ℃解冻,取0.2 g放入EP管中加入纯水混匀,5 000 r/min离心10 min取上清液,用气相色谱法对乙酸、丙酸、丁酸及总SCFAs含量进行测定。

1.3.3 小肠组织切片的制作和观察

于4%甲醛溶液取出小鼠空肠,切成约4 mm的小段放入包埋盒中,水洗过夜,用酒精和二甲苯脱水透明,石蜡浸没包埋,以厚度5 μm切片,展片后贴在载玻片上烘干,二甲苯脱蜡,依次经过浓度从高到低的酒精,苏木素-伊红染色后,脱水透明,用中性树胶进行封固。使用Revolve正倒置一体显微镜观察切片并记录绒毛高度(villus height,VH)、隐窝深度(crypt depth,CD),测量时每个样品选取3个视野,每个视野内取2根绒毛和2个隐窝;根据VH和CD计算绒隐比(VH/CD)。

1.3.4 16S rDNA扩增子测序

将小鼠盲肠内容物样本解冻,采用CTAB法提取样品总基因组DNA。1%琼脂糖凝胶检测DNA浓度和纯度。按浓度用无菌水将DNA稀释至1 ng/μL。利用保守区设计通用引物扩增16S基因的V3~V4区,由北京诺禾致源生物信息技术有限公司在Illumina Nova Seq 6000平台上进行测序。默认以相似度大于97%的序列聚类成为操作分类单元(OTUs),使用Qiime软件(Version 1.9.1)计算Chao1指数、ACE指数、Shannon指数和Simpson指数,分别在门和属水平上统计各样本的群落组成,进行物种注释分析并绘制物种相对丰度柱形图,选择相对丰度排名前10的物种,用相对丰度的平均值来计算在各组中的比例。

1.4 数据统计分析

通过SPSS 21.0分析软件,采用独立样本t检验对2组数据进行处理分析,P<0.05表示差异显著,P<0.01表示差异极显著。表中数据以“平均值±标准误”表示。

2 结果与分析

2.1 植物乳杆菌对小鼠体重的影响

表1可知,与对照组相比,植物乳杆菌组小鼠初始体重、终末体重以及增重率均无显著差异(P>0.05)。
表1 植物乳杆菌对小鼠体重的影响

Table 1 Effects of L. plantarum on body weight of mice

项目
Items
对照组
Control group
植物乳杆菌组
L. plantarum group
P
P-value
初始体重initial body weight/g 22.36±0.26 22.57±0.21 0.536
终末体重final body weight/g 30.79±0.27 31.21±0.34 0.344
增重率WGR/% 38.56±2.10 38.19±2.40 0.910

同行数据肩标无字母表示差异不显著(P>0.05),不同小写字母表示差异显著(P<0.05),不同大写字母表示差异极显著(P<0.01)。下表同。

In the same row, values with no letter superscripts mean no significant difference (P>0.05), while with different small letter superscripts mean significant difference (P<0.05), and with different capital letter superscripts mean extremely significant difference (P<0.01). The same as below.

2.2 植物乳杆菌对小鼠肠道形态的影响

表2可知,与对照组相比,灌胃植物乳杆菌后小鼠空肠VH和CD虽变化不显著(P>0.05),但在数值上VH有所升高、CD有所降低,同时VH/CD显著提高(P<0.05),表明植物乳杆菌可以改善小鼠肠道形态。
表2 植物乳杆菌对小鼠肠道形态的影响

Table 2 Effects of L. plantarum on intestinal morphology of mice

项目
Items
对照组
Control group
植物乳杆菌组
L. plantarum group
P
P-value
绒毛高度VH/μm 320.69±8.25 336.14±7.48 0.171
隐窝深度CD/μm 90.68±2.36 86.52±3.35 0.317
绒隐比VH/CD 23.69±1.75a 30.67±2.24b 0.017

2.3 植物乳杆菌对小鼠血清学指标及盲肠内容物SCFAs含量的影响

表3可知,与对照组相比,灌胃植物乳杆菌后小鼠血清中促炎性细胞因子(CRP、IL-8、TNF-α)的含量无显著差异(P>0.05),但均表现出一定的下降趋势。
表3 植物乳杆菌对小鼠血清学指标的影响

Table 3 Effects of L. plantarum on serological indexes of mice

项目
Items
对照组
Control group
植物乳杆菌组
L. plantarum group
P
P-value
C反应蛋白CRP/(mg/L) 2.12±0.17 2.02±0.17 0.694
白细胞介素-8 IL-8/(ng/L) 34.83±2.28 29.30±2.46 0.174
肿瘤坏死因子-α TNF-α/(ng/L) 27.77±2.26 26.95±2.17 0.630
表4可知,植物乳杆菌组小鼠盲肠内容物中乙酸、丙酸、丁酸含量虽与对照组的差异不显著(P>0.05),但从数值上看均有所增加,同时总SCFAs含量较对照组显著升高(P<0.05)。
表4 植物乳杆菌对小鼠盲肠内容物SCFAs含量的影响

Table 4 Effects of L. plantarum on SCFAs contents in cecal content of mice mg/kg

项目
Items
对照组
Control group
植物乳杆菌组
L. plantarum group
P
P-value
乙酸Acetate 6.85±0.78 8.14±0.84 0.325
丙酸Propionate 2.70±0.29 2.82±0.50 0.796
丁酸Butyrate 1.55±0.21 2.00±0.40 0.221
总短链脂肪酸Total SCFAs 11.78±0.32a 13.61±0.42b 0.025

2.4 植物乳杆菌对小鼠肠道菌群结构的影响

表5可知,与对照组相比,植物乳杆菌组小鼠肠道菌群α多样性指数——Chao1指数、ACE指数、Shannon指数和Simpson指数均无显著差异(P>0.05)。
表5 α多样性指数分析结果

Table 5 Results of α diversity indexes analysis

项目
Items
对照组
Control group
植物乳杆菌组
L. plantarum group
P
P-value
Chao1指数Chao1 index 544.20±7.09 609.66±50.19 0.226
ACE指数ACE index 551.83±9.44 597.47±30.82 0.187
Simpson指数Simpson index 0.98±0.00 0.97±0.01 0.297
Shannon指数Shannon index 6.64±0.08 6.54±0.23 0.703
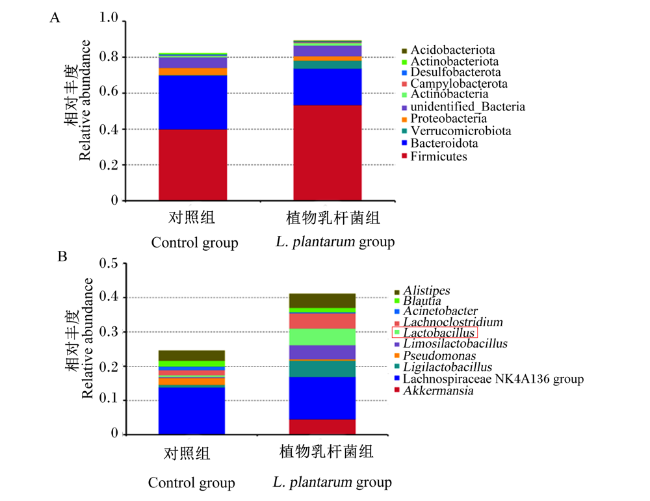
从门水平上分析物种组成(图1-A)发现,2组小鼠肠道菌群以厚壁菌门(Firmicutes)、拟杆菌门(Bacteroidota)、变形菌门(Proteobacteria)为主。对照组中厚壁菌门、拟杆菌门、变形菌门的相对丰度分别占39.99%、30.08%、4.03%,占总数的74.10%;与对照组相比,植物乳杆菌组中变形菌门的相对丰度下降至2.58%,厚壁菌门和拟杆菌门的相对丰度分别上升至53.40%、20.24%。由表6可知,与对照组相比,植物乳杆菌组厚壁菌门的相对丰度显著升高(P<0.05),同时厚壁菌门与拟杆菌门的比值(F/B)有升高的趋势(P=0.057)。在属水平上对物种组成进行分析(图1-B),植物乳杆菌组乳杆菌属(Lactobacillus)的相对丰度与对照组相比极显著升高(P<0.01)。
图1 植物乳杆菌对肠道菌群门和属水平相对丰度的影响

A:在门水平上的物种组成与相对丰度 species composition and relative abundance at phylum level; B:在属水平上的物种组成与相对丰度 species composition and relative abundance at genus level。

Firmicutes:厚壁菌门;Bacteroidota:拟杆菌门;Verrucomicrobiota:疣杆菌门;Proteobacteria:变形菌门;unidentified_Bacteria:未知菌门;Actinobacteriota:放线菌门;Campylobacterota:弯曲菌门;Desulfobacterota:脱硫菌门;Actinobacteria:放线菌门;Acidobacteriota:酸杆菌门;Akkermansia:阿克曼菌属;Lachnospiraceae NK4A136 group:毛螺菌科NK4A136群;Ligilactobacillus:柔韧乳杆菌属;Pseudomonas:假单胞菌属;Limosilactobacillus:罗伊氏乳杆菌属;Lactobacillus:乳杆菌属;Lachnoclostridium:毛螺梭菌;Acinetobacter:不动杆菌属;Blautia:布劳特氏菌属;Alistipes:另枝菌属。

Fig.1 Effects of L. plantarum on relative abundance of intestinal flora at phylum and genus levels of mice

表6 门水平和属水平上肠道菌群相对丰度比较

Table 6 Comparison of relative abundance of intestinal flora at phylum and genus levels

项目
Items
对照组
Control group
植物乳杆菌组
L. plantarum group
P
P-value
厚壁菌门Firmicutes/% 39.99±4.38a 53.40±3.40b 0.035
拟杆菌门Bacteroidota/% 30.08±4.78 20.24±2.77 0.107
厚壁菌门/拟杆菌门F/B 1.57±0.33 3.03±0.59 0.057
乳杆菌属Lactobacillus/% 0.55±0.10A 4.83±1.31B 0.009

3 讨论

植物乳杆菌对酸性环境具有较高的耐受性,更易在胃液和胆盐中存活,一些菌株具有功能特异性[15],摄入适量植物乳杆菌对宿主起到多种益生功能[16-17]。Tong等[18]发现,分别灌胃浓度为108、109和1010 CFU/mL的分离自发酵大白菜植物乳杆菌BW2013,小鼠体重的增长没有显著差异。这与本试验的研究结果一致,在本研究结果中,灌胃浓度109 CFU/mL的植物乳杆菌后小鼠的体重和增重率无显著变化,这可能与8周龄小鼠已基本接近体成熟有关。
小肠绒毛高度和隐窝深度与小肠的吸收能力紧密相关。绒毛高度越高吸收面积越大,小肠养分吸收能力越强;隐窝越浅细胞成熟率越高,通过不断分化细胞来弥补上皮细胞脱落,反映肠道消化吸收功能[19]。提高绒隐比,进而增加肠道吸收面积,可以提升肠道对营养物质的吸收利用率[20]。有研究表明,益生菌可以通过影响肠道形态发育,促进绒毛顶端表面上皮细胞的生长来增强肠道的吸收能力[21-22]。在本试验中,灌胃植物乳杆菌可以使小鼠VH有所升高,CD有所降低,VH/CD显著升高,表明植物乳杆菌可改善小鼠小肠形态结构。Yang等[23]的研究表明,从健康婴儿的粪便中分离出来的植物乳杆菌1258可以预防肠黏膜损伤,改善小肠形态。Suo等[24]在仔猪饲粮中添加源自婴儿粪便的植物乳杆菌ZJ316,发现仔猪肠道VH和CD均有改善。这与本研究结果一致,说明在饲喂基础饲粮的基础上灌胃植物乳杆菌可以增大小鼠肠道VH/CD,进而提高小鼠的消化吸收能力。
TNF-α、IL-8等炎症因子的含量增加可能造成组织损伤引发炎症反应,炎症加剧刺激肝细胞释放CRP[25]。有研究表明植物乳杆菌可显著降低炎症因子的表达[26]。这与本试验结果不同,本试验中灌胃植物乳杆菌后小鼠血清中CRP、IL-8、TNF-α的含量无显著变化,可能是由于小鼠自身特异性、饲粮营养水平、环境等因素造成的,植物乳杆菌是否对机体炎症的发生产生影响有待进一步研究。生物体内微生物消化代谢产生SCFAs[27-28],已有研究证明SCFAs有显著的抗炎作用[29-30],降低部分炎症因子的表达[31]。本试验结果表明,植物乳杆菌组小鼠血清炎症因子含量的变化不显著,但有减少的趋势,植物乳杆菌组盲肠内容物中总SCFAs的含量显著升高。Kamil等[32]的研究表明,添加一种从天然发酵的水牛奶分离的植物乳杆菌Dad-13可增加产生丁酸的菌种丰度,益生菌组的总SCFAs、丙酸和丁酸含量升高。前人的研究结果与本研究结果结合,说明植物乳杆菌单独作用不会引起机体炎症反应,但植物乳杆菌能引起总SCFAs含量升高,为植物乳杆菌通过产生SCFAs、下调炎症因子表达来缓解炎症反应的发生提供了可能。
通常情况下,肠道菌群的紊乱与疾病有关,而干预肠道菌群是否对动物产生积极影响,从而成为一种缓解疾病的措施仍需要进一步研究,因此,本试验利用16S rDNA扩增子测序技术分析植物乳杆菌对小鼠肠道菌群的影响。16S rDNA扩增子测序是一种快速并且相对准确的确定样本中所有微生物遗传信息的技术[33]。Chao1指数和ACE指数反映菌群丰富度,Shannon指数和Simpson指数反映菌群多样性[34]。本试验结果表明,灌胃植物乳杆菌对小鼠肠道菌群丰富度和多样性均没有显著影响,不会造成小鼠的肠道菌群紊乱。任荣[35]发现,短时间内灌胃源自发酵浆水的植物乳杆菌JS5对小鼠肠道菌群α多样性的影响有限,与本试验结果一致。而Bao等[36]研究显示,小鼠肠道菌群α多样性指数中的ACE指数和Chao1指数在添加分离自蒙古酸马奶菌种植物乳杆菌2-33后显著上升,表明植物乳杆菌2-33对小鼠肠道菌群的丰富度具有正向调节作用。在本研究过程中形成该结果的原因可能有这2点:第一,小鼠肠道菌群稳态之前已经形成,可以保持一段时间的稳定性;第二,益生菌有助于恢复有益微生物的正常水平,而不破坏胃肠道的细菌群落组成。
厚壁菌门作为一个重要指标来指示肠道健康[37],而变形菌门相对丰度升高可能诱发炎症反应[38]。本研究结果显示,在小鼠灌胃植物乳杆菌后,厚壁菌门作为优势菌门其相对丰度显著上升,而变形菌门的相对丰度则出现下降趋势。这与王梦美等[39]研究得出的从仿刺参肠道中筛选的植物乳杆菌HMX-3可使仿刺参肠道菌群中厚壁菌门的相对丰度上升、变形菌门的相对丰度下降的结果相似。F/B是提示肠道菌群健康的重要指标,该比值也与SCFAs相关[40]。在本试验中植物乳杆菌组小鼠F/B有上升趋势,这与其总SCFAs含量有显著上升的结果一致。在属水平上的物种分析结果显示植物乳杆菌组小鼠乳杆菌属的相对丰度较对照组极显著上升。有研究表明,乳杆菌属大多为可产生SCFAs的益生菌,其相对丰度与生殖道炎症[41]、抑郁症[42]、结直肠肿瘤的发生[43]等呈负相关。植物乳杆菌可通过黏附于黏膜和上皮,与其他不良细菌成分形成竞争抑制[26]。本研究结果同样证明,植物乳杆菌能通过改变肠道微生物群组成增强肠上皮屏障功能。因此,植物乳杆菌能够有效促进肠道有益菌相对丰度的提高,降低潜在致病菌的相对丰度,促进SCFAs的产生,改善肠道内环境。

4 结论

灌胃植物乳杆菌可提高小鼠空肠绒隐比,改善小鼠肠道吸收功能;对血清炎症因子含量没有显著影响,但可升高盲肠内容物总SCFAs含量,增强肠道屏障功能;使肠道菌群中乳杆菌属等有益菌的相对丰度增加,对有害菌有一定的抑制作用,进而调节肠道菌群,改善肠道内环境。综上可知,植物乳杆菌不仅未使小鼠产生炎症反应,还对其肠道健康具有积极作用。
[1]
ROGGERO P, LIOTTO N, POZZI C, et al. Analysis of immune,microbiota and metabolome maturation in infants in a clinical trial of Lactobacillus paracasei CBA L74-fermented formula[J]. Nature Communications, 2020, 11(1):2703.

DOI

[2]
LI Y T, LIU A F, CHEN L X, et al. Lactobacillus plantarum WSJ-06 alleviates neurobehavioral injury induced by lead in mice through the gut microbiota[J]. Food and Chemical Toxicology, 2022, 167:113308.

DOI

[3]
RAJASEKHARAN S K, SHEMESH M. Spatiotemporal bio-shielding of bacteria through consolidated geometrical structuring[J]. NPJ Biofilms and Microbiomes, 2022, 8(1):37.

DOI PMID

[4]
YANG K M, ZHU C, WANG L, et al. Early supplementation with Lactobacillus plantarum in liquid diet modulates intestinal innate immunity through toll-like receptor 4-mediated mitogen-activated protein kinase signaling pathways in young piglets challenged with Escherichia coli K88[J]. Journal of Animal Science, 2021, 99(6):skab128.

DOI

[5]
SCHWARZER M, MAKKI K, STORELLI G, et al. Lactobacillus plantarum strain maintains growth of infant mice during chronic undernutrition[J]. Science, 2016, 351(6275):854-857.

DOI

[6]
KUDA T, KAWAHARA M, NEMOTO M, et al. In vitro antioxidant and anti-inflammation properties of lactic acid bacteria isolated from fish intestines and fermented fish from the Sanriku Satoumi region in Japan[J]. Food Research International, 2014, 64:248-255.

DOI

[7]
VAN BAARLEN P, TROOST F J, VAN HEMERT S, et al. Differential NF-κB pathways induction by Lactobacillus plantarum in the duodenum of healthy humans correlating with immune tolerance[J]. Proceedings of the National Academy of Sciences of the United States of America, 2009, 106(7):2371-2376.

[8]
梁东梅, 李玉鹏, 杜艳芬, 等. 三株乳酸杆菌的分离鉴定与益生特性研究[J]. 中国饲料, 2018(11):24-29.

LIANG D M, LI Y P, DU Y F, et al. Study on the isolation,identification of three strains of Lactobacilli and their probiotic properties[J]. China Feed, 2018(11):24-29. (in Chinese)

[9]
李海花, 梁东梅, 乔家运. 植物乳杆菌抑制产肠毒素型大肠杆菌诱发猪肠上皮细胞炎症反应的分子机制[J]. 动物营养学报, 2021, 33(7):4018-4029.

DOI

LI H H, LIANG D M, QIAO J Y. Molecular mechanism of Lactobacillus plantarum inhibiting inflammatory response induced by enterotoxigenic Escherichia coli in porcine intestinal epithelial cells[J]. Chinese Journal of Animal Nutrition, 2021, 33(7):4018-4029. (in Chinese)

[10]
OSTOJIC S M. Inadequate production of H2 by gut microbiota and Parkinson disease[J]. Trends in Endocrinology & Metabolism, 2018, 29(5):286-288.

[11]
WANG Y L, WEI J, ZHANG W Y, et al. Gut dysbiosis in rheumatic diseases:a systematic review and meta-analysis of 92 observational studies[J]. EBioMedicine, 2022, 80:104055.

DOI

[12]
JIA Q J, WANG L R, ZHANG X N, et al. Prevention and treatment of chronic heart failure through traditional Chinese medicine:role of the gut microbiota[J]. Pharmacological Research, 2020, 151:104552.

DOI

[13]
王小燕, 翁剑青. 感染性休克患者炎症因子水平变化及其临床价值[J]. 现代医学与健康研究电子杂志, 2022, 6(15):99-102.

WANG X Y, WENG J Q. Changes and clinical value of inflammatory factors in patients with septic shock[J]. Modern Medicine and Health Research Electronic Journal, 2022, 6(15):99-102. (in Chinese)

[14]
TYLICKA M, GUSZCZYN T, MAKSIMOWICZ M, et al. The concentration of selected inflammatory cytokines (IL-6,IL-8,CXCL5,IL-33) and damage-associated molecular patterns (HMGB-1,HSP-70) released in an early response to distal forearm fracture and the performed closed reduction with Kirschner wire fixation in children[J]. Frontiers in Endocrinology, 2021, 12:749667.

DOI

[15]
BIAGIOLI M, CAPOBIANCO D, CARINO A, et al. Divergent effectiveness of multispecies probiotic preparations on intestinal microbiota structure depends on metabolic properties[J]. Nutrients, 2019, 11(2):325.

DOI

[16]
LONG X Y, ZENG X F, TAN F, et al. Lactobacillus plantarum KFY04 prevents obesity in mice through the PPAR pathway and alleviates oxidative damage and inflammation[J]. Food & Function, 2020, 11(6):5460-5472.

[17]
LO CURTO A, PITINO I, MANDALARI G, et al. Survival of probiotic lactobacilli in the upper gastrointestinal tract using an in vitro gastric model of digestion[J]. Food Microbiology, 2011, 28(7):1359-1366.

DOI

[18]
TONG T, NIU X H, LI Q, et al. The effect of Lactobacillus plantarum BW2013 on the gut microbiota in mice analyzed by 16S rRNA amplicon sequencing[J]. Polish Journal of Microbiology, 2021, 70(2):235-243.

DOI

[19]
卫旭彪, 张璐璐, 马广, 等. 酵母菌对猪肠道绒毛、隐窝及菌群的影响[J]. 饲料工业, 2016, 37(4):61-64.

WEI X B, ZHANG L L, MA G, et al. Effects of yeasts on intestinal villus,crypt and flora in pigs[J]. Feed Industry, 2016, 37(4):61-64. (in Chinese)

[20]
SONG J, XIAO K, KE Y L, et al. Effect of a probiotic mixture on intestinal microflora,morphology,and barrier integrity of broilers subjected to heat stress[J]. Poultry Science, 2014, 93(3):581-588.

DOI

[21]
王晓成, 孙亚楠, 任发政, 等. 益生菌对健康小鼠肠道形态发育的影响[J]. 中国奶牛, 2017(6):49-54.

WANG X C, SUN Y N, REN F Z, et al. Effects of probiotics on intestinal morphology in healthy mice[J]. China Dairy Cattle, 2017(6):49-54. (in Chinese)

[22]
COLLADO M C, CERNADA M, BAÜERL C, et al. Microbial ecology and host-microbiota interactions during early life stages[J]. Gut Microbes, 2012, 3(4):352-365.

DOI PMID

[23]
YANG K M, JIANG Z Y, ZHENG C T, et al. Effect of Lactobacillus plantarum on diarrhea and intestinal barrier function of young piglets challenged with enterotoxigenic Escherichia coli K88[J]. Journal of Animal Science, 2014, 92(4):1496-1503.

DOI

[24]
SUO C, YIN Y S, WANG X N, et al. Effects of Lactobacillus plantarum ZJ316 on pig growth and pork quality[J]. BMC Veterinary Research, 2012, 8:89.

DOI

[25]
路钰夏, 杨辉, 王向辉, 等. 病毒感染性腹泻对儿童人群肠道菌群及IL-6、TNF-α、hs-CRP、IFN-γ水平的影响[J]. 中国实验诊断学, 2022, 26(6):842-846.

LU Y X, YANG H, WANG X H, et al. Effect of virus-infected diarrhea on intestinal flora and levels of IL-6,TNF-α,hs-CRP and IFN-γin children[J]. Chinese Journal of Laboratory Diagnosis, 2022, 26(6):842-846. (in Chinese)

[26]
ROCCHETTI M T, RUSSO P, CAPOZZI V, et al. Bioprospecting antimicrobials from Lactiplantibacillus plantarum:key factors underlying its probiotic action[J]. International Journal of Molecular Sciences, 2021, 22(21):12076.

DOI

[27]
FERNANDES J, SU W, RAHAT-ROZENBLOOM S, et al. Adiposity,gut microbiota and faecal short chain fatty acids are linked in adult humans[J]. Nutrition & Diabetes, 2014, 4(6):e121.

[28]
MACHIELS K, JOOSSENS M, SABINO J, et al. A decrease of the butyrate-producing species Roseburia hominis and Faecalibacterium prausnitzii defines dysbiosis in patients with ulcerative colitis[J]. Gut, 2014, 63(8):1275-1283.

DOI

[29]
TEDELIND S, WESTBERG F, KJERRULF M, et al. Anti-inflammatory properties of the short-chain fatty acids acetate and propionate:a study with relevance to inflammatory bowel disease[J]. World Journal of Gastroenterology, 2007, 13(20):2826-2832.

DOI

[30]
ARORA T, BÄCKHED F. The gut microbiota and metabolic disease:current understanding and future perspectives[J]. Journal of Internal Medicine, 2016, 280(4):339-349.

DOI

[31]
WANG Y Q, WU J T, LV M X, et al. Metabolism characteristics of lactic acid bacteria and the expanding applications in food industry[J]. Frontiers in Bioengineering and Biotechnology, 2021, 9:612285.

DOI

[32]
KAMIL R Z, MURDIATI A, JUFFRIE M, et al. Gut microbiota modulation of moderate undernutrition in infants through gummy Lactobacillus plantarum Dad-13 consumption:a randomized double-blind controlled trial[J]. Nutrients, 2022, 14(5):1049.

DOI

[33]
QI H T, LIU Y, QI X, et al. Dietary recombinant phycoerythrin modulates the gut microbiota of H22 tumor-bearing mice[J]. Marine Drugs, 2019, 17(12):665.

DOI

[34]
LV Y, REN G, REN X J. Changes of intestinal flora and lymphocyte subsets in patients with chronic renal failure[J]. Evidence-based Complementary and Alternative Medicine, 2021, 2021:4288739.

[35]
任荣. 两株植物乳杆菌的功能特性及其提升羊酸乳品质研究[D]. 硕士学位论文. 西安: 陕西师范大学, 2021.

REN R. Study on functional characteristics of two strains of Lactobacillus plantarum and their improvement of sheep acid milk quality[D]. Master's Thesis. Xi'an: Shaanxi Normal University, 2021. (in Chinese)

[36]
BAO W Y D I, HE Y X, YU J H, et al. Regulatory effect of Lactiplantibacillus plantarum 2-33 on intestinal microbiota of mice with antibiotic-associated diarrhea[J]. Frontiers in Nutrition, 2022, 9:921875.

DOI

[37]
LI H Q, ZHOU Y, LING H Y, et al. The effect of dietary supplementation with Clostridium butyricum on the growth performance,immunity,intestinal microbiota and disease resistance of tilapia (Oreochromis niloticus)[J]. PLoS One, 2019, 14(12):e0223428.

DOI

[38]
VASQUES-MONTEIRO I M L, SILVA-VEIGA F M, MIRANDA C S, et al. A rise in Proteobacteria is an indicator of gut-liver axis-mediated nonalcoholic fatty liver disease in high-fructose-fed adult mice[J]. Nutrition Research, 2021, 91:26-35.

DOI

[39]
王梦美, 吕成杰, 杨顶珑, 等. 植物乳杆菌(LPHMX-3)对仿刺参生长、消化、免疫和肠道菌群的影响[J/OL]. 水产学报, 2022:1-11.(2022-06-11). http://kns.cnki.net/kcms/detail/31.1283.S.20220609.1517.006.html.

WANG M M, LYU C J, YANG D L, et al. Effects of Lactobacillus plantarum (LP HMX-3) on growth,digestion,immunity and intestinal flora of Apostichopus japonicus[J/OL]. Journal of Fisheries of China, 2022:1-11.(2022-06-11). http://kns.cnki.net/kcms/detail/31.1283.S.20220609.1517.006.html. (in Chinese)

[40]
VAISERMAN A, ROMANENKO M, PIVEN L, et al. Differences in the gut Firmicutes to Bacteroidetes ratio across age groups in healthy Ukrainian population[J]. BMC Microbiology, 2020, 20(1):221.

DOI PMID

[41]
CHEN H L, MIN S L, WANG L, et al. Lactobacillus modulates chlamydia infectivity and genital tract pathology in vitro and in vivo[J]. Frontiers in Microbiology, 2022, 13:877223.

DOI

[42]
SCHAUB A C, SCHNEIDER E, VAZQUEZ-CASTELLANOS J F, et al. Clinical,gut microbial and neural effects of a probiotic add-on therapy in depressed patients:a randomized controlled trial[J]. Translational Psychiatry, 2022, 12(1):227.

DOI

[43]
YAN S H, CHANG J Y, HAO X H, et al. Berberine regulates short-chain fatty acid metabolism and alleviates the colitis-associated colorectal tumorigenesis through remodeling intestinal flora[J]. Phytomedicine, 2022, 102:154217.

DOI

文章导航

/