综述

糖皮质激素与热应激奶牛免疫系统互作机制的研究进展

  • 谭健 ,
  • 余诗强 ,
  • 赵玉超 ,
  • 蒋林树 , *
展开
  • 北京农学院动物科学技术学院,奶牛营养学北京市重点实验室,北京 102206
* 蒋林树,教授,博士生导师,E-mail:

谭健(2000—),男,湖南湘潭人,硕士研究生,研究方向为奶牛营养与免疫。E-mail:

Copy editor: 武海龙

收稿日期: 2023-03-24

  网络出版日期: 2023-09-13

基金资助

家畜产业技术体系北京市创新团队(BAIC05-2022)

中国博士后科学基金资助项目(2022M710181)

Research Progress on Interaction Mechanism between Glucocorticoids and Immune System of Heat Stressed Dairy Cows

  • TAN Jian ,
  • YU Shiqiang ,
  • ZHAO Yuchao ,
  • JIANG Linshu , *
Expand
  • Key Laboratory for Dairy Cow Nutrition, College of Animal Science and Technology, Beijing University of Agriculture, Beijing 102206, China
* professor, E-mail:

Received date: 2023-03-24

  Online published: 2023-09-13

摘要

热应激是影响奶牛生产性能与健康的主要因素之一,奶牛遭受热应激后极易对生产性能、机体代谢和免疫系统产生影响,严重制约了我国奶牛养殖业的健康快速发展。奶牛遭受热应激时,下丘脑-垂体-肾上腺轴被激活,体内糖皮质激素水平发生改变,而糖皮质激素作为奶牛的主要应激激素,具有多种生物学功能,可以调节机体多种免疫功能。本文就热应激期间奶牛体内糖皮质激素对奶牛非特异性免疫和特异性免疫功能的影响进行阐述,旨在为缓解奶牛热应激提供科学依据。

本文引用格式

谭健 , 余诗强 , 赵玉超 , 蒋林树 . 糖皮质激素与热应激奶牛免疫系统互作机制的研究进展[J]. 动物营养学报, 2023 , 35(9) : 5496 -5504 . DOI: 10.12418/CJAN2023.506

Abstract

Heat stress is one of the main factors affecting dairy cows’ performance and health. Heat stress can negatively affect dairy cows’ performance, body metabolism and immune system, seriously restricting the healthy and rapid development of dairy farming industry in China. When dairy cows are subjected to heat stress, the hypothalamus-pituitary-adrenal axis is activated, and the level of glucocorticoids in the body changes. As the primary stress hormone in dairy cows, glucocorticoids have multiple biological functions and can regulate various immune functions. This review summarized the effects of glucocorticoids on nonspecific and specific immune functions of dairy cows during heat stress, providing the scientific basis for alleviating heat stress in dairy cows.

在外界环境变化的刺激下,动物会通过迅速改变体内糖皮质激素水平来应对多种应激源,这种反应引发的生理和行为变化对于应对各种挑战至关重要[1]。糖皮质激素是一类由肾上腺产生的维持机体内稳态的小脂质激素,循环至血液后与靶细胞结合发挥作用,对动物机体发挥多效性作用[2],其水平高低反映了动物的健康程度[3]。皮质醇是糖皮质激素的主要表现形式,并作为反刍动物主要的应激激素[4-5],在动物遭受应激过程中可以紧急调动信号转导通路,合成分泌相关激素及增强机体代谢,且奶牛遭受热应激后生产性能、免疫能力、繁殖效率的下降和感染疾病风险的上升常伴随着奶牛体内皮质醇水平的显著改变[6-7]。此外,糖皮质激素药物如氢化可的松、地塞米松等,可在体内发挥抗炎和免疫调节作用,已被广泛用作免疫抑制剂和抗炎剂来治疗多种自身免疫和炎症性疾病[8]。因此,糖皮质激素作为奶牛应激反应的主要生物学标志物,研究其对奶牛热应激条件下免疫功能影响的调控作用机制,对缓解奶牛热应激、改善奶牛健康状况、维持机体热应激免疫代谢稳态具有重要意义。基于此,本文综述了糖皮质激素与热应激奶牛免疫系统互作机制的国内外研究进展,旨在为下一步的深入研究提供理论支撑。

1 糖皮质激素对奶牛免疫功能的作用机制

反刍动物发生应激反应会促进体内糖皮质激素释放,促进免疫细胞凋亡并干扰其免疫系统功能[9]。免疫系统反应是应对抵御挑战的重要机制,热应激通过影响奶牛体内糖皮质激素分泌,诱导机体免疫反应,产生不同的细胞因子[10]表1列举了不同生理或生长阶段奶牛遭受热应激后血液皮质醇水平和免疫指标的变化。糖皮质激素通过与2种受体结合发出信号,即Ⅰ型盐皮质激素受体(type Ⅰ mineralocorticoid receptors,MRs)和Ⅱ型糖皮质激素受体(type Ⅱ glucocorticoid receptors,GRs)。MRs位于海马、杏仁核、皮层、脑干处细胞的细胞质中,对糖皮质激素有着较高的亲和力,在其浓度较低时几乎与糖皮质激素完全结合[11-12]。GRs则在整个大脑和机体组织中广泛表达,包括垂体前叶和下丘脑-垂体-肾上腺(hypothalamic-pituitary-adrenal,HPA)轴活性区域[13]。GRs在正常生理状态下与糖皮质激素的亲和力较低,但机体遭受热应激体内糖皮质激素水平升高后,GRs被激活并增强与糖皮质激素的结合[14]。糖皮质激素的分子作用包括与GRs结合直接调控一些细胞因子mRNA转录来影响细胞因子的合成,包括白细胞介素(interleukin,IL)-1、IL-2、IL-3、IL-4、IL-5、IL-6、IL-8、IL-12、IL-18、粒细胞-巨噬细胞集落刺激因子(granulocyte-macrophage colony-stimulating factor,GM-CSF)、肿瘤坏死因子-α(tumor necrosis factor-α,TNF-α)和干扰素-γ(interferon-γ,IFN-γ)[15]。此外,糖皮质激素可以导致机体淋巴细胞的凋亡[16],也能通过细胞因子和趋化因子受体促进T细胞和B细胞的存活、重新分布和反应,并增强对某些感染的免疫反应[17]
表1 不同生理或生长阶段奶牛遭受热应激后血液皮质醇水平和免疫指标的变化

Table 1 Changes of blood cortisol level and immune indices at different physiological or growth stages of cows during heat stress

奶牛品种
Cow breeds
生理或生长阶段
Physiological or
growth stages
血液皮质醇水平变化
Change of blood
cortisol level
血液免疫指标变化
Change of blood
immune indices
参考文献
References
荷斯坦 Holstein 产前遭遇热应激后所产犊牛 上升 中性粒细胞计数、单核细胞百分比上升,
淋巴细胞绝对值下降
唐程[18]
荷斯坦 Holstein 产前遭遇热应激后所产犊牛 下降 IgG含量下降 Tao等[19]
荷斯坦 Holstein 犊牛 上升 IgG含量下降 Stott等[20]
印度沙希瓦 India Sahiwal 泌乳期 下降 IL-2、IL-8、IL-10含量下降 Alhussien等[21]
荷斯坦 Holstein 泌乳初期 下降 IL-6、TNF-α含量上升,IgG含量下降 张志登[22]
荷斯坦 Holstein 泌乳中期 上升 IL-1β、TNF-α含量上升,IgG含量下降 张轶凤[23]
荷斯坦 Holstein 泌乳中期 上升 IL-1β、IL-6、IL-8、IL-10、TNF-α
含量上升,IgG含量下降
李蓉[24]
荷斯坦 Holstein 泌乳中期 上升 IL-10、TNF-α、IL-1β、IgG含量上升 Li等[25]

IgG:免疫球蛋白G immunoglobulin G;IL:白细胞介素 interleukin;TNF-α:肿瘤坏死因子-α tumor necrosis factor-α。

2 糖皮质激素在奶牛热应激时期的分泌

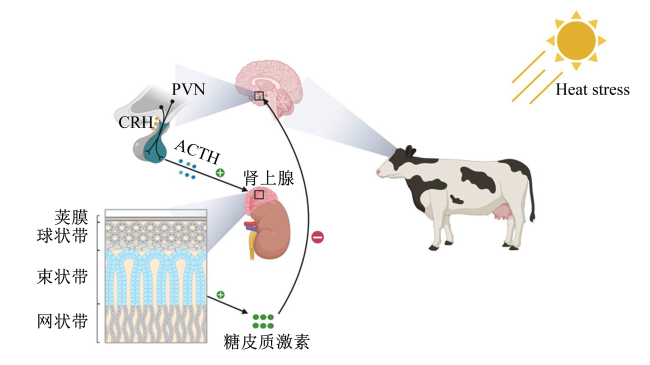
当动物处在稳定的生理状态时,糖皮质激素的产生受昼夜节律控制[17]。白天活动的动物血液中糖皮质激素水平在清晨达到顶峰值,在夜间达到最低值,而在夜间活动的动物如啮齿类动物中则相反。当动物处在应激状态时,体内糖皮质激素分泌量激增。在热应激期间,奶牛HPA轴被激活,以对热应激刺激做出反应,维持机体稳态[26]。奶牛遭受热应激时,体内HPA轴、下丘脑-垂体-甲状腺(hypothalamic-pituitary-thyroid,HPT)轴和下丘脑-垂体-性腺(hypothalamic-pituitary-gonad,HPG)轴被刺激启动,其中HPA轴的激活在缓解奶牛热应激影响中至关重要[27]。下丘脑脑室旁核(paraventricular nucleus,PVN)作为HPA轴的起点,在受到外界刺激时其神经元释放促肾上腺皮质激素释放激素(corticotropin releasing hormone,CRH)和精氨酸加压素(arginine vasopressin,AVP),释放的CRH与垂体前叶的CRH受体结合,激活前阿片皮质激素(proopiomelanocortin,POMC)的产生,然后将其转化为促肾上腺皮质激素(adrenocorticotropic hormone,ACTH)释放到循环中[28]。ACTH通过全身循环进入肾上腺皮质并与肾上腺皮质束状带中的特定细胞表面G蛋白耦联受体,即黑素皮质素-2型受体(melanocortin type-2 receptor,MC2R)结合后,糖皮质激素类固醇生成被激活[29]。在肾上腺皮质束状带细胞内线粒体中,胆固醇受到一系列类固醇生成调节剂的酶促修饰,最终合成糖皮质激素释放到全身[30]。同时,糖皮质激素可以在下丘脑和垂体前叶进行负反馈调节,减少CRH和ACTH的分泌,抑制HPA轴应激活性[31]图1为热应激期间奶牛体内糖皮质激素分泌的示意图。根据奶牛遭受热应激的持续天数,热应激可分为短期热应激和长期热应激。短期热应时期,奶牛HPA轴被激活,糖皮质激素合成释放增加,体内皮质醇水平升高,对免疫系统产生刺激作用[32]。长期热应激时期,奶牛HPA轴被长期激活受损,糖皮质激素合成释放减少,造成体内皮质醇水平降低,并产生免疫抑制[33-34]
图1 热应激期间奶牛体内糖皮质激素分泌的示意图

Heat stress:热应激;PVN:下丘脑脑室旁核 paraventricular nucleus;CRH:促肾上腺皮质激素释放激素 corticotropin releasing hormone;ACTH:促肾上腺皮质激素 adrenocorticotropic hormone。

Fig.1 Diagrammatic sketch of glucocorticoids secretion of dairy cows during heat stress

3 糖皮质激素对奶牛非特异性免疫的作用

非特异性免疫又称先天性免疫或固有免疫,是机体暴露于感染或免疫时立即起作用的第1道防线,包括物理屏障、固有免疫细胞和固有免疫因子。当机体的物理屏障无法消除病原体时,免疫系统会通过促进中性粒细胞、血液中的单核细胞和组织中的巨噬细胞等转移到感染部位来做出反应[35]。白细胞是免疫系统的主要组成部分,可分为中性粒细胞、嗜酸性粒细胞、嗜碱性粒细胞、单核细胞、淋巴细胞,不同种类的白细胞以不同的方式参与机体防御反应,其主要功能是保护机体免受细菌、病毒、真菌和寄生虫等入侵的传染性病原体的侵害。研究表明,短暂的急性热应激会改变初生犊牛的白细胞总数和免疫功能[36]。吞噬细胞(中性粒细胞和巨噬细胞)介导的非特异性免疫反应直到妊娠晚期才发育完全,临近分娩时,胎儿体内皮质酮水平升高,导致中性粒细胞的吞噬和杀菌能力下降[37]。奶牛的白细胞数量在热应激条件下受到影响,与其他季节相比,夏季荷斯坦奶牛血液中白细胞总数显著降低[38]。干奶期遭受过热应激的奶牛,在泌乳早期的平均白细胞计数和中性粒细胞计数显著降低,所产犊牛的血清中性粒细胞计数、淋巴细胞百分比显著下降,皮质醇水平与单核细胞百分比显著上升[18]

3.1 中性粒细胞

中性粒细胞是多形核和颗粒状白细胞,是先天免疫系统抵御入侵微生物的第1道防线[39]。体内激素水平或代谢功能变化会导致奶牛免疫功能下降,并进一步导致不同程度的免疫抑制,造成奶牛中性粒细胞趋化性、跨上皮迁移的速度和吞噬作用下降[40]。奶牛临近产犊时,由于胎儿皮质醇水平的升高,中性粒细胞的吞噬和杀菌能力下降[37]。Narayan等[41]研究表明,遭受夏季热应激的奶牛血液内中性粒细胞数量显著降低。然而,糖皮质激素调节中性粒细胞凋亡的机制尚不清楚。糖皮质激素介导中性粒细胞凋亡的机制可能包括上调凋亡B细胞淋巴瘤-2凋亡基因(B-cell lymphoma-2,Bcl-2)和凋亡抑制剂家族成员。例如,地塞米松可以通过中性粒细胞中的磷脂酰肌醇3-激酶(phosphatidylinositol 3-kinase,PI3K)和p38丝裂原激活蛋白激酶(mitogen-activated protein kinases,MAPK)诱导存活,并增强Bcl-2家族的促凋亡成员髓样细胞白血病-1(myeloid cell leukemia-1,MCL-1)表达[42]。糖皮质激素可以促进巨噬细胞吞噬凋亡的白细胞,并使其快速降解,且不会引起促炎性反应[43]。此外,糖皮质激素可以抑制中性粒细胞的在体内的活化与迁移。Ricci等[44]研究发现,糖皮质激素诱导亮氨酸拉链(glucocorticoids-induced leucine zipper,GILZ)通过控制膜联蛋白A1的表达来抑制中性粒细胞的迁移。GILZ还能通过抑制MAPK途径和中性粒细胞分泌促炎因子,抑制中性粒细胞向炎症部位的活化与迁移[45]。糖皮质激素可以降低细胞因子、趋化因子和黏附因子的表达,抑制白细胞与内皮细胞的相互作用,导致中性粒细胞的黏附与转移能力下降[46]

3.2 巨噬细胞

巨噬细胞是由血液中的单核细胞穿出血管后分化而成,不仅在非特性免疫中发挥作用,还充当连接非特异性免疫和特异性免疫的桥梁,具有激活T细胞和B细胞的作用[47]。糖皮质激素受体激活,可以刺激单核细胞分化为抗炎组织吞噬细胞[48]。Joo等[49]研究发现,处于夏季热应激的荷斯坦奶牛,外周血液单核细胞数量呈下降趋势。另一项研究表明,体外暴露于高温环境下的奶牛外周血单核细胞凋亡增加,同时细胞活力降低[50]。热应激条件下,糖皮质激素对奶牛体内单核细胞的外渗调节作用尚不明确。而低水平糖皮质激素对巨噬细胞功能(如黏附、转化、吞噬和细胞因子产生)有免疫刺激作用,高水平糖皮质激素对巨噬细胞有免疫抑制作用[51-52]。Dong等[53]研究表明,高水平皮质醇通过调节核因子-κB(nuclear factor-κB,NF-κB)和MAPK信号通路,减弱了RAW264.7巨噬细胞系中脂多糖(lipopolysaccharide,LPS)诱导的炎症反应。糖皮质激素药物地塞米松可以诱导GRs向Krüppel样转录因子9启动子聚集,增加线粒体活性氧(reactive oxygen species,ROS)产生,导致巨噬细胞线粒体依赖性凋亡[54]

4 糖皮质激素对奶牛特异性免疫的作用

特异性免疫由细胞免疫和体液免疫组成,又称获得性免疫或适应性免疫,主要由免疫球蛋白和免疫淋巴细胞与抗原结合引起特异性免疫[55]。淋巴细胞主要由B细胞和T细胞组成,参与各种免疫功能,如免疫球蛋白的产生和细胞因子的产生对免疫应答的调节[56]。T细胞主要参与细胞免疫,B细胞在体液免疫中发挥重要作用。许多研究发现,在夏季高温或热应激发生时,奶牛体内淋巴细胞的数量显著降低[57-59]

4.1 细胞免疫

热应激通过增加绵羊体内皮质醇水平而损害细胞免疫反应,皮质醇与DNA结合,抑制参与T细胞活化和细胞因子产生的基因表达[60-61]。当动物受到应激时,糖皮质激素可以抑制T细胞前体细胞在胸腺成熟和诱导淋巴细胞凋亡的途径,使血液中淋巴细胞的数量降低[62]。辅助性T细胞(helper T cells,Th细胞)是T细胞的一种,是特异性免疫的重要参与者。热应激期间奶牛淋巴细胞功能受损可能与细胞免疫降低有关,这会影响Th-1细胞和Th-2细胞平衡,有利于Th-2细胞因子的分泌,最终影响淋巴细胞增殖[63]。糖皮质激素可以优先抑制Th-1细胞和Th-17细胞的反应,同时保留甚至促进Th-2细胞和调节性T细胞的功能[46]。体外研究表明,热应激会对有丝分裂原刀豆球蛋白A(concanavalin A,Con A)刺激的奶牛外周血单核细胞产生影响,对淋巴细胞的增殖具有抑制作用[59]。Xing等[64]提出,糖皮质激素可以诱导活化T细胞中的程序性死亡细胞-1(programmed cell death-1,PD-1)表达,并抑制T细胞受体(T cell receptor,TCR)介导的T细胞增殖和IL-2、IFN-γ和TNF-α等细胞因子产生。地塞米松可以抑制细胞因子的分泌并诱导其凋亡,从而影响T细胞活性[65]。糖皮质激素对于T细胞的免疫抑制包括其抑制T细胞增殖和细胞因子产生以及对细胞凋亡的诱导[66]

4.2 体液免疫

B细胞是来源于骨髓的多能干细胞,在抗原的刺激下可分化为记忆细胞和产生抗体(免疫球蛋白)的浆细胞来执行机体的体液免疫,浆细胞分泌的免疫球蛋白可以分为5类:免疫球蛋白G(IgG)、免疫球蛋白M(IgM)、免疫球蛋白A(IgA)、免疫球蛋白E(IgE)、免疫球蛋白D(IgD),通常检测IgG、IgM、IgA含量来判断机动物的体液免疫功能。Godden[67]研究发现,奶牛在妊娠后期遭受热应激会降低初乳质量,IgG、IgA含量显著降低,总蛋白、酪蛋白、乳清蛋白、乳脂肪和乳糖含量减少。干奶期遭受热应激的经产荷斯坦奶牛,在产犊后90 d内的产奶量以及乳中IgG含量显著降低[68]。遭受热应激的犊牛血清中IgG含量也低于凉爽环境中的犊牛[19]。遭受热应激的母牛在在妊娠后期血液中IgG含量升高,非热应激组的小母牛由于血液中的抗体转移到初乳中,IgG含量降低,这可能表明热应激对奶牛母体免疫球蛋白向初乳的转移有负面影响[69]。处于热应激状态的奶牛体内皮质酮水平升高,诱导细胞发生长时间的溶解反应,使得奶牛体内免疫球蛋白合成量降低,最终导致免疫功能下降[10]
GRs存在于从动物骨髓和脾脏分离出来的B细胞群体中,单日多次注射氢化可的松可以调节B细胞的产生[70],且单日多次注射地塞米松可以调节骨髓中的未成熟B细胞数量,但不会影响体内成熟B细胞的数量[71]。动物应激相关的B细胞减少是由于高水平的糖皮质激素导致前体B细胞从骨髓中产生时发生凋亡[72],糖皮质激素可以调节成熟B细胞在血液和骨髓之间的每日交换,且血液中B细胞数量与糖皮质激素水平呈负相关[73]。此外,糖皮质激素可在体内和体外增强B细胞中IgE的产生,而无需抗原挑战,在B细胞中具有选择性免疫刺激作用[74]。目前,糖皮质激素对B细胞功能影响的研究较少,多数集中于糖皮质激素对动物遭受应激反应后体内球蛋白的影响,而遭受热应激的奶牛体液免疫功能的变化与糖皮质激素水平升高的相关机制值得进一步研究。

5 小结

糖皮质激素通过与不同受体结合影响奶牛的非特异性免疫和特异性免疫,在维持奶牛免疫功能中发挥重要作用。奶牛遭受不同程度的热应激可造成体内糖皮质激素水平改变,短期热应激奶牛体内糖皮质激素水平升高对奶牛产生免疫刺激作用,长期热应激奶牛免疫系统被遭受破坏,体内糖皮质激素水平下降可引发免疫抑制作用。因此,体内糖皮质激素有可能作为奶牛热应激状态的生物学标志物,有待进一步验证。未来通过体内外试验探究糖皮质激素与免疫系统的相互作用,可为营养调控改善热应激对奶牛免疫功能提供新思路。
[1]
VITOUSEK M N, TAFF C C, RYAN T A, et al. Stress resilience and the dynamic regulation of glucocorticoids[J]. Integrative and Comparative Biology, 2019, 59(2):251-263.

DOI PMID

[2]
TAVES M D, ASHWELL J D. Glucocorticoids in T cell development,differentiation and function[J]. Nature Reviews Immunology, 2021, 21(4):233-243.

DOI

[3]
ROMERO L M, BEATTIE U K. Common myths of glucocorticoid function in ecology and conservation[J]. Journal of Experimental Zoology Part A:Ecological and Integrative Physiology, 2022, 337(1):7-14.

DOI

[4]
BINSIYA T K, SEJIAN V, BAGATH M, et al. Significance of hypothalamic-pituitary-adrenal axis to adapt to climate change in livestock[J]. International Research Journal of Agricultural and Food Sciences, 2017, 2(1):1-20.

[5]
WOJTAS K, CWYNAR P, KOŁACZ R. Effect of thermal stress on physiological and blood parameters in merino sheep[J]. Journal of Veterinary Research, 2014, 58(2):283-288.

[6]
POLSKY L, VON KEYSERLINGK M A G. Invited review:effects of heat stress on dairy cattle welfare[J]. Journal of Dairy Science, 2017, 100(11):8645-8657.

DOI

[7]
ZACHUT M, KRA G, LIVSHITZ L, et al. Seasonal heat stress affects adipose tissue proteome toward enrichment of the Nrf2-mediated oxidative stress response in late-pregnant dairy cows[J]. Journal of Proteomics, 2017, 158:52-61.

DOI PMID

[8]
JIA W Y, ZHANG J J. Effects of glucocorticoids on leukocytes:genomic and non-genomic mechanisms[J]. World Journal of Clinical Cases, 2022, 10(21):7187-7194.

DOI

[9]
张千, 李发弟, 李飞. 反刍动物应激反应中糖皮质激素对免疫系统的调节机理[J]. 畜牧兽医学报, 2017, 48(5):785-792.

ZHANG Q, LI F D, LI F. Regulation mechanism of glucocorticoids to immune system in ruminants stress response[J]. Acta Veterinaria et Zootechnica Sinica, 2017, 48(5):785-792. (in Chinese)

[10]
BAGATH M, KRISHNAN G, DEVARAJ C, et al. The impact of heat stress on the immune system in dairy cattle:a review[J]. Research in Veterinary Science, 2019, 126:94-102.

DOI

[11]
DE KLOET E R, REUL J M, SUTANTO W. Corticosteroids and the brain[J]. The Journal of Steroid Biochemistry and Molecular Biology, 1990, 37(3):387-394.

DOI

[12]
LE MENUET D, LOMBÈS M. The neuronal mineralocorticoid receptor:from cell survival to neurogenesis[J]. Steroids, 2014, 91:11-19.

DOI

[13]
HAN F, OZAWA H, MATSUDA K I, et al. Colocalization of mineralocorticoid receptor and glucocorticoid receptor in the hippocampus and hypothalamus[J]. Neuroscience Research, 2005, 51(4):371-381.

PMID

[14]
WEIKUM E R, KNUESEL M T, ORTLUND E A, et al. Glucocorticoid receptor control of transcription:precision and plasticity via allostery[J]. Nature Reviews Molecular Cell Biology, 2017, 18(3):159-174.

DOI

[15]
SHIMBA A, IKUTA K. Control of immunity by glucocorticoids in health and disease[J]. Seminars in Immunopathology, 2020, 42(6):669-680.

DOI PMID

[16]
BREWER J A, KANAGAWA O, SLECKMAN B P, et al. Thymocyte apoptosis induced by T cell activation is mediated by glucocorticoids in vivo[J]. The Journal of Immunology, 2002, 169(4):1837-1843.

DOI

[17]
SHIMBA A, EJIMA A, IKUTA K. Pleiotropic effects of glucocorticoids on the immune system in circadian rhythm and stress[J]. Frontiers in Immunology, 2021, 12:706951.

DOI

[18]
唐程. 干奶期母牛热应激对母牛和犊牛生长、生产性能及血液生化指标的影响[D].硕士学位论文. 扬州: 扬州大学, 2020.

TANG C. Effects of heat stress on growth,production performance and blood biochemical indexes of cows and calves during dry milk period[D].Master’s Thesis. Yangzhou: Yangzhou University, 2020. (in Chinese)

[19]
TAO S, MONTEIRO A P A, THOMPSON I M, et al. Effect of late-gestation maternal heat stress on growth and immune function of dairy calves[J]. Journal of Dairy Science, 2012, 95(12):7128-7136.

DOI PMID

[20]
STOTT G H, WIERSMA F, MENEFEE B E, et al. Influence of environment on passive immunity in calves[J]. Journal of Dairy Science, 1976, 59(7):1306-1311.

PMID

[21]
ALHUSSIEN M N, DANG A K. Integrated effect of seasons and lactation stages on the plasma inflammatory cytokines,function and receptor expression of milk neutrophils in Sahiwal (Bos indicus) cows[J]. Veterinary Immunology and Immunopathology, 2017, 191:14-21.

DOI

[22]
张志登. 热应激对宁夏地区泌乳奶牛生产性能及血液生化指标的影响[D].硕士学位论文. 银川: 宁夏大学, 2019.

ZHANG Z D. Effects of heat stress on production performance and blood biochemical parameters of lactating dairy cows in Ningxia[D].Master’s Thesis. Yinchuan: NingXia University, 2019. (in Chinese)

[23]
张轶凤. 南方荷斯坦奶牛冷热应激评价指标及适宜环境温湿度研究[D].硕士学位论文. 武汉: 华中农业大学, 2019.

ZHANG Y F. Evaluation index and suitable environment temperature and humidity for cold and heat stress of Holstein cows in South China[D].Master’s Thesis. Wuhan: Huazhong Agricultural University, 2019. (in Chinese)

[24]
李蓉. 高温高湿对泌乳奶牛生产性能和粪样菌群的影响及喷淋效果研究[D].硕士学位论文. 武汉: 华中农业大学, 2018.

LI R. Effects of high temperature-humidity and spray measures on production performance and fecal bacterial communities in lactating cows[D].Master’s Thesis. Wuhan: Huazhong Agricultural University, 2018. (in Chinese)

[25]
LI H, ZHANG Y F, LI R, et al. Effect of seasonal thermal stress on oxidative status,immune response and stress hormones of lactating dairy cows[J]. Animal Nutrition, 2021, 7(1):216-223.

DOI

[26]
SEJIAN V, BHATTA R, GAUGHAN J B, et al. Review:adaptation of animals to heat stress[J]. Animal, 2018, 12(S2):s431-s444.

DOI

[27]
刘嘉莉, 窦金焕, 胡丽蓉, 等. 热应激对奶牛生理和免疫功能的影响及其机理[J]. 中国畜牧兽医, 2018, 45(1):263-270.

LIU J L, DOU J H, HU L R, et al. Effects and mechanism of heat stress on physiological and immune system in dairy cows[J]. China Animal Husbandry&Veterinary Medicine, 2018, 45(1):263-270. (in Chinese)

[28]
STEPHENS M A C, WAND G. Stress and the HPA axis:role of glucocorticoids in alcohol dependence[J]. Alcohol Research:Current Reviews, 2012, 34(4):468-483.

[29]
MOUNTJOY K G, MORTRUD M T, LOW M J, et al. Localization of the melanocortin-4 receptor (MC4-R) in neuroendocrine and autonomic control circuits in the brain[J]. Molecular Endocrinology, 1994, 8(10):1298-1308.

PMID

[30]
HUM D W, MILLER W L. Transcriptional regulation of human genes for steroidogenic enzymes[J]. Clinical Chemistry, 1993, 39(2):333-340.

PMID

[31]
PACKARD A E B, EGAN A E, ULRICH-LAI Y M. HPA axis interactions with behavioral systems[J]. Comprehensive Physiology, 2016, 6(4):1897-1934.

DOI PMID

[32]
GELLRICH K, SIGL T, MEYER H H D, et al. Cortisol levels in skimmed milk during the first 22 weeks of lactation and response to short-term metabolic stress and lameness in dairy cows[J]. Journal of Animal Science and Biotechnology, 2015, 6(1):31.

DOI

[33]
GRELET C, VANDEN DRIES V, LEBLOIS J, et al. Identification of chronic stress biomarkers in dairy cows[J]. Animal, 2022, 16(5):100502.

DOI

[34]
SAFA S, KARGAR S, MOGHADDAM G A, et al. Heat stress abatement during the postpartum period:effects on whole lactation milk yield,indicators of metabolic status,inflammatory cytokines,and biomarkers of the oxidative stress[J]. Journal of Animal Science, 2019, 97(1):122-132.

[35]
INBARAJ S, SEJIAN V, BAGATH M, et al. Impact of heat stress on immune responses of livestock:a review[J]. Pertanika Journal of Tropical Agricultural Science, 2016, 39(4):459-482.

[36]
STRONG R A, SILVA E B, CHENG H W, et al. Acute brief heat stress in late gestation alters neonatal calf innate immune functions[J]. Journal of Dairy Science, 2015, 98(11):7771-7783.

DOI PMID

[37]
BARRINGTON G M, PARISH S M. Bovine neonatal immunology[J]. Veterinary Clinics of North America:Food Animal Practice, 2001, 17(3):463-476.

DOI

[38]
BHAN C, SINGH S V, HOODA O K, et al. Influence of temperature variability on physiological,hematological and biochemical profiles of growing and adult Karan Fries cattle[J]. Indian Journal of Animal Sciences, 2013, 83(10):1090-1096.

[39]
MAYADAS T N, CULLERE X, LOWELL C A. The multifaceted functions of neutrophils[J]. Annual Review of Pathology:Mechanisms of Disease, 2014, 9:181-218.

DOI

[40]
LV G X, WANG H, ZHOU X C, et al. Effects of hormone,NEFA and SCFA on the migration of neutrophils and the formation of neutrophil extracellular traps in dairy cows[J]. Animals, 2022, 12(9):1190.

DOI

[41]
NARAYAN U, SINGH D V, SHARMA R J. Physiological responses in holstein-friesian crossbred lactating cows under heat stress ameliorating treatments[J]. Indian Journal of Animal Research, 2007, 41(2):130-133.

[42]
HIRSCH G, LAVOIE-LAMOUREUX A, BEAUCHAMP G, et al. Neutrophils are not less sensitive than other blood leukocytes to the genomic effects of glucocorticoids[J]. PLoS One, 2012, 7(9):e44606.

DOI

[43]
CHAPMAN K E, COUTINHO A, GRAY M, et al. Local amplification of glucocorticoids by 11β-hydroxysteroid dehydrogenase type 1 and its role in the inflammatory response[J]. Annals of the New York Academy of Sciences, 2006, 1088(1):265-273.

DOI

[44]
RICCI E, RONCHETTI S, PERICOLINI E, et al. Role of the glucocorticoid-induced leucine zipper gene in dexamethasone-induced inhibition of mouse neutrophil migration via control of annexin A1 expression[J]. The FASEB Journal, 2017, 31(7):3054-3065.

DOI

[45]
RICCI E, RONCHETTI S, GABRIELLI E, et al. GILZ restrains neutrophil activation by inhibiting the MAPK pathway[J]. Journal of Leukocyte Biology, 2019, 105(1):187-194.

DOI PMID

[46]
CAIN D W, CIDLOWSKI J A. Immune regulation by glucocorticoids[J]. Nature Reviews Immunology, 2017, 17(4):233-247.

DOI PMID

[47]
SORDILLO L M, SHAFER-WEAVER K, DEROSA D. Immunobiology of the mammary gland[J]. Journal of Dairy Science, 1997, 80(8):1851-1865.

DOI PMID

[48]
HEIDEVELD E, HAMPTON-O’NEIL L A, CROSS S J, et al. Glucocorticoids induce differentiation of monocytes towards macrophages that share functional and phenotypical aspects with erythroblastic island macrophages[J]. Haematologica, 2018, 103(3):395-405.

DOI PMID

[49]
JOO S S, LEE S J, PARK D S, et al. Changes in blood metabolites and immune cells in Holstein and Jersey dairy cows by heat stress[J]. Animals, 2021, 11(4):974.

DOI

[50]
CATOZZI C, ÁVILA G, ZAMARIAN V, et al. In-vitro effect of heat stress on bovine monocytes lifespan and polarization[J]. Immunobiology, 2020, 225(2):151888.

DOI

[51]
ZEN M, CANOVA M, CAMPANA C, et al. The kaleidoscope of glucorticoid effects on immune system[J]. Autoimmunity Reviews, 2011, 10(6):305-310.

DOI PMID

[52]
LIM H Y, MÜLLER N, HEROLD M J, et al. Glucocorticoids exert opposing effects on macrophage function dependent on their concentration[J]. Immunology, 2007, 122(1):47-53.

DOI

[53]
DONG J S, LI A A, CUI L Y, et al. Cortisol modulates inflammatory responses in LPS-stimulated RAW264.7 cells via the NF-κB and MAPK pathways[J]. BMC Veterinary Research, 2018, 14(1):30.

DOI PMID

[54]
AI F L, ZHAO G H, LV W, et al. Dexamethasone induces aberrant macrophage immune function and apoptosis[J]. Oncology Reports, 2020, 43(2):427-436.

DOI PMID

[55]
ELENKOV I J. Neurohormonal-cytokine interactions:implications for inflammation,common human diseases and well-being[J]. Neurochemistry International, 2008, 52(1/2):40-51.

DOI

[56]
TRINCHIERI G, PFLANZ S, KASTELEIN R A. The IL-12 family of heterodimeric cytokines:new players in the regulation of T cell responses[J]. Immunity, 2003, 19(5):641-644.

DOI

[57]
ELVINGER F, HANSEN P J, NATZKE R P. Modulation of function of bovine polymorphonuclear leukocytes and lymphocytes by high temperature in vitro and in vivo[J]. American Journal of Veterinary Research, 1991, 52(10):1692-1698.

[58]
KAMWANJA L A, CHASE C C,Jr, GUTIERREZ J A, et al. Responses of bovine lymphocytes to heat shock as modified by breed and antioxidant status[J]. Journal of Animal Science, 1994, 72(2):438-444.

PMID

[59]
LACETERA N, BERNABUCCI U, SCALIA D, et al. Heat stress elicits different responses in peripheral blood mononuclear cells from Brown Swiss and Holstein cows[J]. Journal of Dairy Science, 2006, 89(12):4606-4612.

PMID

[60]
CAROPRESE M, ALBENZIO M, BRUNO A, et al. Effects of shade and flaxseed supplementation on the welfare of lactating ewes under high ambient temperatures[J]. Small Ruminant Research, 2012, 102(2/3):177-185.

DOI

[61]
SGORLON S, COLITTI M, ASQUINI E, et al. Administration of botanicals with the diet regulates gene expression in peripheral blood cells of Sarda sheep during ACTH challenge[J]. Domestic Animal Endocrinology, 2012, 43(3):213-226.

DOI PMID

[62]
RODRIGUES-MASCARENHAS S, DOS SANTOS N F, RUMJANEK V M. Synergistic effect between ouabain and glucocorticoids for the induction of thymic atrophy[J]. Bioscience Reports, 2006, 26(2):159-169.

DOI

[63]
LACETERA N, BERNABUCCI U, SCALIA D, et al. Lymphocyte functions in dairy cows in hot environment[J]. International Journal of Biometeorology, 2005, 50(2):105-110.

PMID

[64]
XING K L, GU B X, ZHANG P, et al. Dexamethasone enhances programmed cell death 1 (PD-1) expression during T cell activation:an insight into the optimum application of glucocorticoids in anti-cancer therapy[J]. BMC Immunology, 2015, 16:39.

DOI

[65]
OKOYE I S, XU L, WALKER J, et al. The glucocorticoids prednisone and dexamethasone differentially modulate T cell function in response to anti-PD-1 and anti-CTLA-4 immune checkpoint blockade[J]. Cancer Immunology Immunotherapy, 2020, 69(8):1423-1436.

DOI

[66]
BOLDIZSAR F, TALABER G, SZABO M, et al. Emerging pathways of non-genomic glucocorticoid (GC) signaling in T cells[J]. Immunobiology, 2010, 215(7):521-526.

DOI

[67]
GODDEN S. Colostrum management for dairy calves[J]. Veterinary Clinics of North America:Food Animal Practice, 2008, 24(1):19-39.

DOI

[68]
ADIN G, GELMAN A, SOLOMON R, et al. Effects of cooling dry cows under heat load conditions on mammary gland enzymatic activity,intake of food and water,and performance during the dry period and after parturition[J]. Livestock Science, 2009, 124(1/3):189-195.

DOI

[69]
NARDONE A, LACETERA N, BERNABUCCI U, et al. Composition of colostrum from dairy heifers exposed to high air temperatures during late pregnancy and the early postpartum period[J]. Journal of Dairy Science, 1997, 80(5):838-844.

PMID

[70]
DA COSTA K M, VALENTE R C, DA SILVA J M C, et al. Glucocorticoid susceptibility and in vivo ABCB1 activity differ in murine B cell subsets[J]. Anais da Academia Brasileira de Ciências, 2018, 90(3):3081-3097.

DOI

[71]
GRUVER-YATES A L, QUINN M A, CIDLOWSKI J A. Analysis of glucocorticoid receptors and their apoptotic response to dexamethasone in male murine B cells during development[J]. Endocrinology, 2014, 155(2):463-474.

DOI

[72]
MCGREGOR B A, MURPHY K M, ALBANO D L, et al. Stress,cortisol,and B lymphocytes:a novel approach to understanding academic stress and immune function[J]. Stress-the International Journal on the Biology of Stress, 2016, 19(2):185-191.

DOI

[73]
CAIN D W, BORTNER C D, DIAZ-JIMENEZ D, et al. Murine glucocorticoid receptors orchestrate B cell migration selectively between bone marrow and blood[J]. The Journal of Immunology, 2020, 205(3):619-629.

DOI

[74]
LIM J, LIN E V, HONG J Y, et al. Induction of natural IgE by glucocorticoids[J]. Journal of Experimental Medicine, 2022, 219(10):e20220903.

DOI

文章导航

/