综述

柚皮苷的生物学功能及其在畜牧生产中的应用

  • 李留学 ,
  • 赵玉超 ,
  • 余诗强 ,
  • 蒋林树 , *
展开
  • 北京农学院动物科学技术学院,奶牛营养学北京市重点实验室,北京 102206
*蒋林树,教授,博士生导师,E-mail:

李留学(1996—),男,河南驻马店人,硕士研究生,从事奶牛营养与免疫研究。E-mail:

Office editor: 田艳明

收稿日期: 2023-04-10

  网络出版日期: 2023-10-12

基金资助

现代农业产业技术体系北京市家畜创新团队

北京市博士后科研活动经费资助(2022-ZZ-129)

Biological Functions of Naringin and Its Application in Livestock Production

  • LI Liuxue ,
  • ZHAO Yuchao ,
  • YU Shiqiang ,
  • JIANG Linshu , *
Expand
  • Key Laboratory for Dairy Cow Nutrition, College of Animal Science and Technology, Beijing University of Agriculture, Beijing 102206, China
*professor, E-mail:

Received date: 2023-04-10

  Online published: 2023-10-12

摘要

在饲料“禁抗”背景下,寻找和开发各种抗生素替代品成为畜牧业亟待解决的重大问题。柚皮苷(NAR)作为一种天然的黄酮类化合物,具有抗氧化、抗炎、抗肿瘤以及改善糖和脂代谢等多种生物学功能,可能成为一种替代抗生素的饲料添加剂。本文针对目前NAR的研究,从理化性质、生物学功能及其在畜牧生产中的应用进行综述,以期为NAR在畜禽生产中的应用和推广提供理论参考。

本文引用格式

李留学 , 赵玉超 , 余诗强 , 蒋林树 . 柚皮苷的生物学功能及其在畜牧生产中的应用[J]. 动物营养学报, 2023 , 35(10) : 6257 -6268 . DOI: 10.12418/CJAN2023.575

Abstract

Under the background of “no antibiotic” in feed, finding and developing various antibiotic substitutes has become an important problem to be solved urgently in animal husbandry. Naringin (NAR) is a subclass of flavonoids, which has many biological functions such as antioxidation, anti-inflammation, anti-tumor and improving glucose and lipid metabolism, and may become a feed additive instead of antibiotics. In this paper, the physical and chemical properties, biological functions and applications of NAR in livestock production were reviewed, in order to provide theoretical references for the application and popularization of NAR in livestock production.

除中药外的所有促生长类药物饲料添加剂被禁用后,我国饲料行业进入“无抗”时代,寻找新的饲料添加剂替代抗生素成为畜牧业关注的热点。天然植物提取物因其来源广、毒副作用小以及具有多种生物活性作用成为替抗产品的潜在候选物,并引起广泛关注。柚皮苷(naringin,NAR)是柑橘类水果中主要的生物活性多酚,其具有抗氧化[1]、抗炎[2]、抗肿瘤[3]以及调节糖和脂代谢[4]等多种生物学活性。欧盟委员会于2012年发布法规,批准NAR作为所有动物饲料添加剂,并于2023年进行了授权续期。但目前关于NAR在畜牧生产中的研究相对较少,阻碍了其作为饲料添加剂在生产中的应用和推广。因此,本文就NAR的理化性质、生物学功能以及在畜牧生产中的应用进行综述,旨在为其饲用化研究提供理论参考。

1 NAR的来源、结构及理化性质

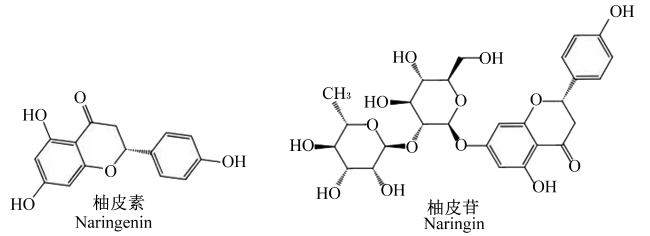
NAR又称柚苷、柑橘苷和异橙皮苷,主要存在于柠檬、橙子和葡萄柚等多种柑橘类水果的果皮和果肉中,同时也是骨碎补[5]、化橘红[6]和枳壳[7]等中药的主要药效成分。NAR最早于1857年在柚子树花中被发现,但直到1928年其化学结构才被首次阐明,其由2个鼠李糖单元连接在其苷元(柚皮素)C-7位置[8-10](图1)。NAR为一种淡黄色结晶性粉末,味苦,常温下在水中的溶解度仅为0.1%,易溶于甲醇、乙醇和稀碱溶液中,不溶于乙醚、己烷和氯仿等非极性溶剂[11]
图1 NAR的结构

Fig.1 Structure of NAR

2 NAR的生物学功能及其作用机制

2.1 抗氧化功能

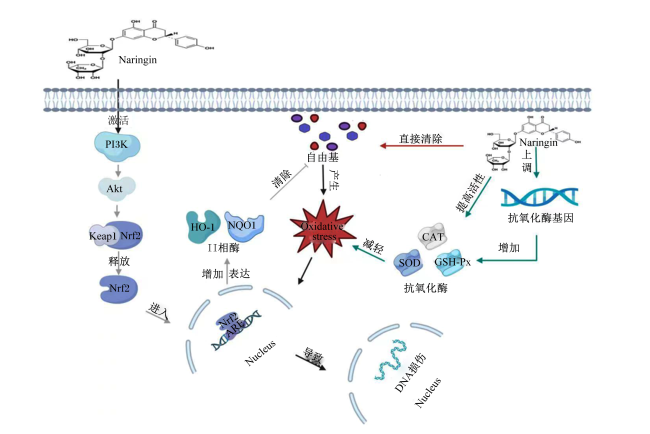
NAR具有较强的抗氧化能力。研究发现,NAR(0.5 g/kg)抗氧化能力可与商用抗氧化剂普罗布考(0.5 g/kg)和洛伐他汀(0.3 g/kg)相媲美[12-13]。NAR可直接清除自由基,减少机体氧化应激的发生。研究发现,NAR清除羟基自由基和2,2'-联氮-双-3-乙基苯并噻唑啉-6-磺酸自由基的半抑制浓度分别为0.32和0.39 mg/mL,而且其清除羟基自由基的能力比抗氧化剂2,6-二叔丁基-4-甲基苯酚更强[14]。同时,NAR对超氧阴离子自由基和2,2-联苯基-1-苦基肼基也具有显著的清除能力[15]。NAR也可提高内源性抗氧化酶的活性,减轻氧化应激损伤。体外试验表明,NAR显著改善了因缺氧/复氧导致H9C2细胞中超氧化物歧化酶(superoxide dismutase,SOD)、过氧化氢酶(catalase,CAT)和谷胱甘肽过氧化物酶(glutathione peroxidase,GSH-Px)活性的降低,其还显著降低了细胞内活性氧(reactive oxygen species,ROS)和丙二醛(malondialdehyde,MDA)的水平,减少了氧化应激损伤[16]。体内试验也发现,NAR通过提高SOD和CAT活性,上调SODCATGSH-Px基因的表达,在调节机体抗氧化能力中发挥重要作用[13]。NAR还参与调控氧化应激信号通路,增强机体抗氧化防御能力。核因子E2相关因子2(nuclear factor E2-related factor 2,Nrf2)是抗氧化信号通路的关键调节因子,负责调控Ⅱ相解毒酶和抗氧化酶基因的协调和表达,而NAR通过磷酸肌醇3激酶(phosphatidylinositol 3 kinase,PI3K)/蛋白激酶B(protein kinase B,Akt)信号通路激活Nrf2,提高受Nrf2调控的抗氧化蛋白血红素加氧酶-1(heme oxygenase-1,HO-1)和还原型烟酰胺腺嘌呤二核苷酸磷酸醌氧化还原酶1[NAD(P)H quinone oxidoreductase 1,NQO1]的表达,减少机体氧化损伤[17-18]。此外,另有研究发现,NAR还可通过激活单磷酸腺苷活化蛋白激酶(AMP-activated kinase,AMPK)/Nrf2途径减轻体外氧化应激[19]。综上可知,NAR一方面通过直接清除自由基,拮抗自由基对细胞的攻击;另一方面通过提高机体内源性抗氧化酶活性,缓解机体氧化应激;此外,NAR还可通过激活抗氧化信号通路,增强机体抗氧化防御系统(图2)。
图2 NAR的抗氧化机制

Naringin:柚皮苷;PI3K:磷酸肌醇3激酶 phosphatidylinositol 3 kinase;Akt:蛋白激酶B protein kinase B;Keap1:Kelch样环氧氯丙烷相关蛋白1 Kelch-like epichlorohydrin-associated protein 1;Nrf2:核因子E2相关因子2 nuclear factor E2-related factor 2;ARE:抗氧化反应元件 antioxidant response element;HO-1:血红素加氧酶-1 heme oxygenase-1;NQO1:还原型烟酰胺腺嘌呤二核苷酸磷酸醌氧化还原酶1 NAD(P)H quinone oxidoreductase 1;Nucleus:细胞核;Oxidative stress:氧化应激;CAT:过氧化氢酶 catalase;SOD:超氧化物歧化酶 superoxide dismutase;GSH-Px:谷胱甘肽过氧化物酶 glutathione peroxidase。

Fig.2 Antioxidant mechanism of NAR[13-16,19]

2.2 抗炎功能

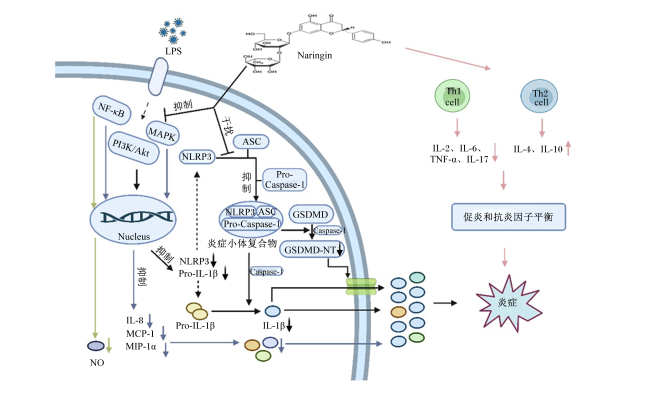
炎症是一种先天的免疫机制,是免疫反应的一个组成部分。但炎症过度或不受控的情况下,会损害宿主组织并引起机体损伤。目前,已有大量研究表明,NAR在动物气道炎症[20-21]、肝炎[22]、关节炎[23]及结肠炎[24]等炎症疾病中发挥抗炎及缓解炎症损伤作用。在小鼠腹膜炎模型中,NAR显著逆转了卡拉胶引起的炎症过程所导致的腹膜液中辅助型T细胞1细胞因子白细胞介素(interleukin,IL)-2、IL-6、肿瘤坏死因子-α(tumor necrosis factor-α,TNF-α)和IL-17水平的升高,并刺激了腹膜液中辅助型T细胞2细胞因子IL-4和IL-10的分泌[25];该研究还表明,NAR处理可降低肺组织中诱导型一氧化氮合酶(inducible nitric oxide synthase,iNOS)、环氧合酶-2(cyclooxygenase-2,COX-2)、细胞黏附分子-1和巨噬细胞炎性蛋白-2等炎性介质的mRNA表达水平,并显著升高转化生长因子-β1的mRNA表达水平[25]。以上研究表明,NAR不仅通过重新调整促炎和抗炎细胞因子释放之间的平衡来诱导其抗炎作用,而且还在基因表达上影响这些细胞因子的平衡。研究发现,芸香柚皮苷显著抑制脂多糖(lipopolysaccharide,LPS)/ATP刺激的巨噬细胞中促炎因子IL-6、IL-1β和TNF-α的分泌[26]。芸香柚皮苷还可抑制LPS/ATP刺激的巨噬细胞中NOD样受体蛋白3(NOD-like receptor protein 3,NLRP3)介导的促炎过程[IL-1β的成熟、活化的半胱氨酸天冬氨酸蛋白酶(Caspase)-1的产生、凋亡相关斑点样蛋白(apoptosis-associated speck-like protein,ASC)的寡聚化及gasdermin D-N末端(GSDMD-NT)的产生和焦亡][26]。此外,NAR还通过抑制核因子-κB(nuclear factor-κB,NF-κB)、丝裂原活化蛋白激酶(mitogen activated protein kinase,MAPK)和PI3K/Akt信号通路抑制LPS诱发的NLRP3和IL-1β表达,并通过干扰NLRP3和ASC之间的相互作用抑制NLRP3炎性小体组装,发挥抗炎作用[26]。NAR还可通过抑制炎症信号通路发挥抗炎功能。Liu等[27]研究表明,NAR通过干扰NF-κB和MAPK信号通路显著抑制了LPS诱导的趋化因子IL-8、单核细胞趋化蛋白-1(monocyte chemotactic protein-1,MCP-1)和巨噬细胞炎症蛋白-1α(macrophage inflammatory protein-1α,MIP-1α)的分泌,并呈剂量依赖性显著降低LPS诱导的IL-8、MCP-1和MIP-1α的mRNA表达。此外,NAR还通过抑制NF-κB的活化减少LPS诱导的一氧化氮(NO)的产生[28]。综上可知,NAR可通过调整促炎和抗炎细胞因子释放之间的平衡,抑制NLRP3途径介导的促炎过程和促炎因子的释放,抑制炎症信号通路发挥抗炎功能(图3)。
图3 NAR的抗炎机制

Naringin:柚皮苷;LPS:脂多糖 lipopolysaccharide;NF-κB:核因子-κB nuclear factor-κB;NO:一氧化氮 nitric oxide;MAPK:丝裂原活化蛋白激酶 mitogen activated protein kinase;PI3K:磷酸肌醇3激酶 phosphatidylinositol 3 kinase;Akt:蛋白激酶B protein kinase B;Nucleus:细胞核;IL-8:白细胞介素-8 interleukin-8;MCP-1:单核细胞趋化蛋白-1 monocyte chemotactic protein-1;MIP-1α:巨噬细胞炎症蛋白-1α macrophage inflammatory protein-1α;NLRP3:NOD样受体蛋白3 NOD-like receptor protein 3;Pro-IL-1β:白细胞介素-1β前体 interleukin-1β precursor;ASC:凋亡相关斑点样蛋白 apoptosis-associated speck-like protein;Pro-Caspase-1:半胱氨酸天冬氨酸蛋白酶1前体 cysteine aspartate protease 1 precursor;Caspase-1:半胱氨酸天冬氨酸蛋白酶1 cysteine aspartate protease 1;GSDMD:gasdermin D;GSDMD-NT:gasdermin D-N末端 gasdermin D-N terminal;IL-1β:白细胞介素-1β interleukin-1β;Th1 cell:辅助型T细胞1 T helper cell 1;Th2 cell:辅助型T细胞2 T helper cell 2;IL-2:白细胞介素-2 interleukin-2;IL-6:白细胞介素-6 interleukin-6;TNF-α:肿瘤坏死因子-α tumor necrosis factor-α;IL-17:白细胞介素-17 interleukin-17;IL-4:白细胞介素-4 interleukin-4;IL-10:白细胞介素-10 interleukin-10。

Fig.3 Anti-inflammatory mechanism of NAR[25-28]

2.3 抗肿瘤功能

近年来研究发现,NAR具有良好的抗癌作用,有希望成为预防和治疗癌症的候选化合物[29]。一方面,NAR通过干扰细胞周期,诱导癌细胞凋亡。NAR通过降低磷酸β-连环蛋白(Ser675)和磷酸糖原合酶激酶-3β(Ser9)的表达和磷酸化阻断β-连环蛋白信号通路,同时增加细胞周期检查点蛋白P21/cip和P27/kip的表达,触发宫颈癌细胞周期停滞在G0/G1期,阻断癌细胞分裂[30]。在胃癌细胞中同样发现NAR阻断癌细胞周期,诱导胃癌细胞凋亡[31]。另一方面,NAR通过外源性和内源性途径介导癌症细胞凋亡。Banjerdpongchai等[32]研究表明,NAR通过激活线粒体介导的Caspase-9和Caspase-8介导的促凋亡因子Bid蛋白的水解,诱导肝癌HepG2细胞凋亡。Ramesh等[33]研究发现,NAR通过死亡受体和线粒体途径增加促凋亡基因Caspasep53、B细胞淋巴瘤-2相关X蛋白(B-cell lymphoma 2-associated X protein,Bax)、Fas死亡受体及其衔接蛋白Fas相关死亡域蛋白(Fas associated death domain protein,FADD)的表达诱导SiHa宫颈癌细胞凋亡。NAR可通过信号通路介导的自噬诱导癌症细胞凋亡。NAR通过阻断PI3K/Akt信号通路,增加微管相关蛋白1轻链3B-Ⅱ和自噬相关蛋白Beclin1的表达以及减少p62的表达激活自噬,诱导胃癌细胞凋亡[34]。NAR还可通过激活MAPK抑制PI3K/Akt/哺乳动物雷帕霉素靶蛋白(mammalian target of rapamycin,mTOR)信号通路诱导自噬,发挥其抗AGS胃癌细胞的增殖活性[35]。此外,NAR通过阻断MAPK信号通路的激活,降低基质金属蛋白酶的表达和活性,抑制胶质瘤U87细胞的侵袭、迁移和黏附作用[36]。除以上途径外,NAR还可通过抑制新生血管的形成,减少癌细胞侵袭和转移,以及与抗癌药物联合应用,抑制癌细胞生长并减弱抗癌药物的副作用[37-38]

2.4 调节血糖代谢功能

NAR通过调节碳水化合物分解酶的活性干扰体内碳水化合物代谢。α-淀粉酶和α-葡萄糖苷酶是动物体内负责催化碳水化合物分解产生单糖以供机体吸收的酶,在医学领域常通过抑制α-淀粉酶和α-葡萄糖苷酶活性,延缓机体对碳水化合物的吸收,降低餐后血糖水平[39]。研究发现,NAR可显著抑制α-淀粉酶和α-葡萄糖苷酶活性,且都呈浓度依赖性[40]。另一项研究同样表明,NAR显著抑制了α-淀粉酶和α-葡萄糖苷酶的活性,且其对2种酶的半抑制浓度作用效果高于降糖药阿卡波糖[41]。因此,NAR可被认为是一种有效的餐后高血糖调节的天然化合物。NAR也可通过调节肝脏糖酵解和糖异生限速酶的活性,控制葡萄糖进入循环,进而调控机体血糖水平。研究表明,NAR通过显著降低肝脏葡萄糖-6-磷酸酶、磷酸烯醇式丙酮酸羧化酶的活性和升高肝脏葡萄糖激酶活性,进而调控糖异生和糖酵解,改善2型糖尿病db/db小鼠的高血糖[42]。另有研究表明,NAR抑制了磷酸烯醇式丙酮酸羧化酶和葡萄糖-6-磷酸酶的mRNA表达,显著上调了葡萄糖激酶的mRNA水平,改善了2型糖尿病小鼠的高血脂症和高血糖[43]。胰岛素是一种降糖激素,通过促进葡萄糖摄取、抑制肝糖异生来维持机体葡萄糖稳态,而胰岛素抵抗是一种无法对胰岛素刺激做出反应的病理状态,导致细胞内糖代谢紊乱[44]。研究发现,NAR可以剂量依赖性地改善胰岛素缺陷型糖尿病小鼠的高血糖,通过抑制内源性和外源性途径抵消链脲霉素诱导的β细胞凋亡且这种保护作用与抑制DNA损伤、NF-κB和MAPK介导的信号传导途径有关[45]。此外,NAR还可改善高脂饮食诱导和2型糖尿病大鼠模型的胰岛素抵抗,调节机体血糖水平[46-47]

2.5 调节脂质代谢功能

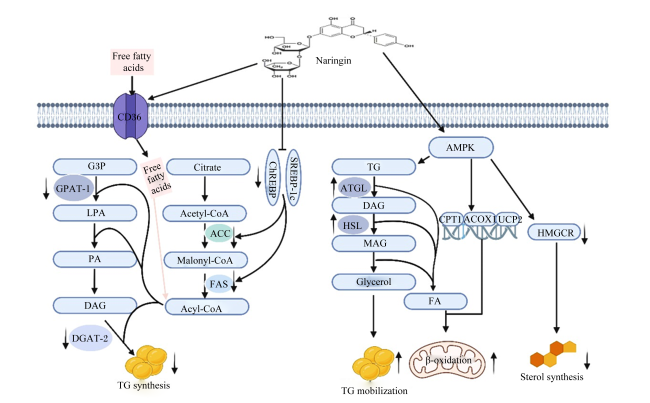
脂质从头生成和甘油-3-磷酸(glycerin-3-phosphate,G3P)途径是机体甘油三酯合成的重要途径,乙酰辅酶A羧化酶(acetyl-CoA carboxylase,ACC)、脂肪酸合成酶(fatty acid synthetase,FAS)、甘油-3-磷酸酰基转移酶-1(glycerol-3-phosphate acyltransferase-1,GPAT-1)和二酰基甘油酰基转移酶-2(diacylglycerol acyltransferase-2,DGAT-2)分别是脂质从头生成和G3P途径的限速酶[48-50]。研究发现,NAR可逆转果糖喂养大鼠肝脏中碳水化合物反应元件结合蛋白(carbohydrate response element binding protein,ChREBP)、甾醇调节元件结合蛋白-1c(sterol regulatory element binding protein-1c,SREBP-1c)表达的增加,以及它们下游靶点ACCFAS的表达上调,同时降低GPAT-1和DGAT-2的蛋白水平,抑制脂质从头生成和G3P途径,减少肝脏中甘油三酯产生[51]。NAR通过激活AMPK的mRNA水平及蛋白磷酸化表达,显著抑制其下游ACCFASSREBP-1c的mRNA及蛋白表达,抑制脂质合成[52]。Zhang等[53]研究发现,NAR还可通过下调白细胞分化抗原36(leukocyte differentiation antigen 36,CD36)和ACC降低脂肪酸的摄取和新生脂肪的生成。
AMPK被认为是细胞能量传感器和脂质代谢的调节器,在脂解过程中调节脂解基因激素敏感脂肪酶(hormone-sensitive lipase,HSL)和脂肪甘油三酯脂酶(adipose triglyceride lipase,ATGL)的表达,控制脂质降解[54]。AMPK在脂肪酸β-氧化中可上调过氧化物酶体增殖物激活受体(peroxisome proliferator activated receptor α,PPARα)调控的下游基因肉毒碱棕榈酰转移酶1(carnitine palmitoyl transferase 1,CPT1)和酰基辅酶A氧化酶1(acyl-CoA oxidase 1,ACOX1)诱导脂肪酸β-氧化[55]。研究发现,NAR处理可增强肥胖小鼠AMPK的激活,显著提高脂肪组织中脂解限速酶HSL和ATGL的蛋白表达,上调小鼠组织中与脂肪酸β-氧化相关基因CPT1、ACOX1和解偶联蛋白2(uncoupling protein 2,UCP2)的表达,表明NAR通过促进脂肪分解和脂肪酸β-氧化有助于减少脂肪堆积[4]。NAR还可通过增加AMPK和ACC的磷酸化,降低3-羟基3-甲基戊二酰辅酶A还原酶(3-hydroxy 3-methylglutaryl CoA reductase,HMGCR)的表达从而降低3T3-L1脂肪细胞的脂质积累和甘油三酯含量[56]。因此,NAR可通过降低脂质从头生成和G3P途径中关键酶活性及脂肪酸的摄取减少脂质合成,提高脂解途径中酶活性及脂肪酸β-氧化水平促进脂质分解,从而调节机体脂质代谢(图4)。
图4 NAR调节脂质代谢的机制

Naringin:柚皮苷;Free fatty acids:游离脂肪酸;CD36:白细胞分化抗原36 leukocyte differentiation antigen 36;G3P:甘油-3-磷酸 glycerin-3-phosphate;GPAT-1:甘油-3-磷酸酰基转移酶-1 glycerol-3-phosphate acyltransferase-1;LPA:溶血磷脂酸 lysophosphatidic acid;PA:磷脂酸 phosphatidic acid;DAG:二酰甘油 diacylglycerol;DGAT-2:二酰基甘油酰基转移酶-2 diacylglycerol acyltransferase-2;TG synthesis:甘油三酯合成 triglyceride synthesis;Citrate:柠檬酸盐;Acetyl-CoA:乙酰辅酶A;ACC:乙酰辅酶A羧化酶 acetyl-CoA carboxylase;Malonyl-CoA:丙二酰辅酶A;FAS:脂肪酸合成酶 fatty acid synthetase;Acyl-CoA:酰基辅酶A;ChREBP:碳水化合物反应元件结合蛋白 carbohydrate response element binding protein;SREBP-1c:甾醇调节元件结合蛋白-1c sterol regulatory element binding protein-1c;TG:甘油三酯 triglyceride;ATGL:脂肪甘油三酯脂酶 adipose triglyceride lipase;MAG:单甘酯 monoglyceride;Glycerol:甘油;TG mobilization:甘油三酯动员 triglyceride mobilization;FA:脂肪酸 fatty acid;AMPK:单磷酸腺苷活化蛋白激酶 AMP-activated kinase;CPT1:肉毒碱棕榈酰转移酶1 carnitine palmitoyl transferase 1;ACOX1:酰基辅酶A氧化酶1 acyl-CoA oxidase 1;UCP2:解偶联蛋白2 uncoupling protein 2;β-oxidation:β-氧化;HMGCR:3-羟基3-甲基戊二酰辅酶A还原酶 3-hydroxy 3-methylglutaryl CoA reductase;Sterol synthesis;固醇合成。

Fig.4 Mechanism of NAR regulates lipid metabolism[4,51-53,56]

3 NAR在畜牧生产中的应用

3.1 NAR在家禽生产中的应用

3.1.1 NAR对家禽生长性能的影响

饲粮中添加NAR不仅可提高鸡的生长性能,而且可保护机体免受有毒、有害物质导致的鸡机体损伤。研究发现,在农药福美双诱导的胫骨软骨发育不良的肉鸡饲粮中添加30 mg/kg NAR,不仅可通过下调印第安刺猬蛋白、上调甲状旁腺激素相关肽mRNA和蛋白的表达恢复受损胫骨的发育,而且能够提高肉鸡的采食量和平均日增重;此外,NAR还可提高肝脏抗氧化能力,减轻肉鸡肝脏损伤[57]。Ebirim等[58]研究表明,饲粮中添加80和160 mg/kg NAR显著提高了小公鸡的体重。此外,NAR还显著提高了醋酸铅毒性诱导的公鸡体重下降,缓解了铅中毒导致的GSH-Px、谷胱甘肽巯基转移酶(glutathione S-transferase,GST)和SOD活性下降,并改善了公鸡的抗氧化防御系统及血清NO的生物利用度[58]。胚蛋注射NAR的研究中发现,17.5 d胚龄的胚蛋注射30 mg NAR可显著增加蛋中孵化小鸡的体重和体长,降低胚胎晚期死亡率[59]。然而,Goliomytis等[60]研究发现,饲粮中添加0.75和1.5 g/kg NAR对肉鸡的体重及胴体和内脏质量无显著影响。NAR导致鸡在促增重方面的差异可能归因于不同品种和不同的添加剂量,因此还需进一步研究。

3.1.2 NAR对家禽繁殖性能和产品品质的影响

研究发现,饲粮中添加NAR显著提高了产蛋后期三黄鸡的血清雌激素水平以及雌激素受体蛋白和基因的表达水平,提高了卵黄前体物形成中的关键基因的转录水平,以及通过增加抗氧化物、减少氧化产物,上调肝脏组织中抗氧化基因的转录水平,增强肝脏抗氧化能力来促进卵黄前体的形成和运输[61]。另一项研究表明,饲粮中添加0.1%、0.2%和0.4%的NAR 8周后,可降低产蛋后期三黄种鸡的料蛋比,提高产蛋率和蛋重,改善蛋黄颜色[62]。此外,饲粮中添加0.2%和0.4%的NAR均可提产蛋后期三黄鸡排卵前的排卵数、生长卵泡数、卵巢指数和卵巢体细胞增殖率,且这种作用可能是由于NAR提高了三黄种鸡抗氧化能力,减轻了氧化应激引起的卵泡闭锁[62]。Bao等[63]证实了NAR能够缓解氧化应激诱导的小白卵泡闭锁,并通过降低氧化应激维持衰老母鸡的产蛋性能。除以上生长和繁殖性能外,饲粮中添加NAR还可提高鸡蛋和屠宰后鸡胴体的抗氧化能力,延长畜产品的货架期。研究表明,NAR能通过减少饱和脂肪酸和增加多不饱和脂肪酸含量改善肉鸡脂肪酸谱,且其对脂肪酸的作用可能是通过调节肝脏中PPARαACOX1的表达来增加脂肪酸β-氧化而介导的[64]。在肉鸡饲粮中添加1.5 g/kg NAR对鸡肉的pH、肉色、剪切力和蒸煮损失无影响,却显著降低了鸡肉储存期间(4 ℃下6和9 d,-20 ℃下120 d)MDA的含量,并且其抗氧化效果与维生素E相当[60]。此外,在蛋鸡饲粮中添加0.75 g/kg NAR,提高了鸡蛋的氧化稳定性,延长了鸡蛋的货架期,并可改善蛋黄颜色[65]

3.2 NAR在猪生产中的应用

NAR可提高仔猪的生产性能,改善育肥猪肉品质和氧化稳定性。在仔猪饲粮中添加NAR可显著提高整个试验期(25~66日龄)的体重和饲料转化率,提高仔猪的生产性能[66]。此外,NAR还显著提高了磷、丙氨酸、天冬氨酸、亮氨酸、赖氨酸和总氨基酸的表观盲肠前消化率[66]。在育肥猪饲粮中添加0.5 g/kg NAR显著提高了猪的眼肌面积和瘦肉含量,且添加剂量为1.5 g/kg时显著提高了背最长肌pH45 min、肌苷酸含量以及SOD活性和总抗氧化能力,并提高了肝脏SOD和GSH-Px活性[67],表明NAR不仅可改善育肥猪的胴体特性,还可提高猪肉氧化稳定性和品质。此外,在猪里脊肉中添加1、3、5和7 g/kg的NAR改变了肉色的光学指标,并且添加5 g/kg NAR可显著提高猪肉的亮度和红度值,降低黄度值,改善新鲜感官度[68]

3.3 NAR在反刍动物生产中的应用

反刍动物生产常通过提高饲粮的精料比例来提高生产性能。然而,高精料常导致瘤胃pH下降,并引起瘤胃酸中毒等一系列代谢性疾病。因此,如何缓解高精料造成代谢性疾病的发生是反刍动物生产中面临的重大问题。研究发现,在高精料饲粮中添加0.5 g/kg NAR显著提高了山羊瘤胃pH和丁酸比例,降低了戊酸比例和乳酸浓度,缓解了因高精料饲粮导致的瘤胃内环境稳态失衡和瘤胃酸中毒[69]。此外,NAR还显著降低了山羊血清IL-6和淀粉样蛋白A含量,缓解了高精料饲粮诱导的炎症反应,显著提高了血清GSH-Px活性,降低了血清MDA含量,改善了高精料饲粮诱发的氧化应激[69]。Balcells等[70]同样研究证明,饲粮中添加生物黄酮(主成分为NAR)可有效改善饲喂高精料饲粮的小母牛瘤胃发酵,并降低瘤胃酸中毒的发生率。
热应激可降低动物体抗氧化状态和免疫反应并引起机体氧化应激和炎症,降低反刍动物生产性能[71-72]。Alhidary等[73]研究发现,给予热应激羔羊7 g/周NAR,显著提高了羔羊的平均日增重和饲料转化效率,改善了羔羊的生产性能;给予14 g/周NAR显著提高了血浆SOD和GSH-Px活性,增强了机体的抗氧化状态。此外,补充NAR增加了注射植物血凝素24 h后羔羊的皮褶厚度,改善了机体细胞免疫[73]
反刍动物饲粮中添加NAR还可提高肉和乳的抗氧化能力。研究发现,羔羊饲粮中添加2.5 g/kg的NAR对肉的pH、肉色、持水力、剪切力和蒸煮损失均无显著影响,但延缓了冷藏条件下羔羊胸最长肌中的脂肪氧化,提高了肉的抗氧化能力[74]。此外,在母羊饲粮中添加6 g/kg NAR提高了羊乳的氧化稳定性,且作用效果与维生素E相当,并对乳样的化学成分、凝固特性和脂肪酸组成无影响[75]

4 小结

在“无抗”背景下,NAR作为天然植物饲料原料陈皮、枳壳和骨碎补的主要成分,不仅具有多种生物学功能,而且可提高畜禽的生产性能、繁殖性能和改善畜产品品质,可见其具有较好的应用前景。但目前关于NAR在畜禽生产中的研究相对较少,且集中在家禽生产上,在猪和反刍动物上的研究匮乏。这就导致NAR在畜禽生产中的研究不够系统和深入,不能明确同品种不同生长阶段或不同品种畜禽的最适添加剂量及作用效果。因此,未来应加强开展NAR在畜禽生产上的研究,为饲料禁抗背景下NAR在畜禽生产上的应用和推广提供依据。
[1]
AKAMO A J, AKINLOYE D I, UGBAJA R N, et al. Naringin prevents cyclophosphamide-induced erythrocytotoxicity in rats by abrogating oxidative stress[J]. Toxicology Reports, 2021, 8:1803-1813.

DOI PMID

[2]
HASSAN R A, HOZAYEN W G, ABO SREE H T, et al. Naringin and hesperidin counteract diclofenac-induced hepatotoxicity in male Wistar rats via their antioxidant,anti-inflammatory,and antiapoptotic activities[J]. Oxidative Medicine and Cellular Longevity, 2021, 2021:9990091.

[3]
STABRAUSKIENE J, KOPUSTINSKIENE D M, LAZAUSKAS R, et al. Naringin and naringenin:their mechanisms of action and the potential anticancer activities[J]. Biomedicines, 2022, 10(7):1686.

DOI

[4]
WANG J, WANG Q, ZHU S Y, et al. Naringin reduces fat deposition by promoting the expression of lipolysis and β-oxidation related genes[J]. Obesity Research & Clinical Practice, 2023, 17(1):74-81.

[5]
YU X, ZHANG P, TANG K, et al. Network pharmacology integrated with molecular docking explores the mechanisms of naringin against osteoporotic fracture by regulating oxidative stress[J]. Evidence-Based Complementary and Alternative Medicine, 2021, 2021:6421122.

[6]
ZENG X, SU W W, LIU B M, et al. A review on the pharmacokinetic properties of naringin and its therapeutic efficacies in respiratory diseases[J]. Mini-Reviews in Medicinal Chemistry, 2020, 20(4):286-293.

DOI

[7]
YUAN J B, WEI F T, LUO X Z, et al. Multi-component comparative pharmacokinetics in rats after oral administration of Fructus aurantii extract,naringin,neohesperidin,and naringin-neohesperidin[J]. Frontiers in Pharmacology, 2020, 11:933.

DOI

[8]
RANGASWAMI S, SESHADRI T R, VEERARAGHAVIAH J. Constitution of naringin:the position of the sugar group[J]. Indian Academy of Sciences, 1939, 9(4):328-332.

[9]
ASAHINA Y, INUBUSE M. Über die konstitution des naringenins (Ⅱ.Mitteilung über die flavanon-glucoside)[J]. European Journal of Inorganic Chemistry, 1928, 61(7):1514-1516.

[10]
ALAM M, AHSAN F, MAHMOOD T, et al. Meticulous parade on naringin respecting its pharmacological activities and novel formulations[J]. Avicenna Journal of Phytomedicine, 2022, 12(5):457-474.

DOI PMID

[11]
许鹭. 柚皮中柚皮苷的提取、分离纯化及其固体分散体与卵磷脂复合物的制备及表征[D]. 硕士学位论文. 广州: 华南理工大学, 2015.

XU L. Extraction and purification of naringin in grapefruit peel and preparation and characterization of its solid dispersion and lecithin compound[D]. Master’s Thesis. Guangzhou: South China University of Technology, 2015. (in Chinese)

[12]
JEON S M, BOK S H, JANG M K, et al. Comparison of antioxidant effects of naringin and probucol in cholesterol-fed rabbits[J]. Clinica Chimica Acta, 2002, 317(1/2):181-190.

DOI

[13]
JEON S M, BOK S H, JANG M K, et al. Antioxidative activity of naringin and lovastatin in high cholesterol-fed rabbits[J]. Life Sciences, 2001, 69(24):2855-2866.

DOI PMID

[14]
AKAMO A J, ROTIMI S O, AKINLOYE D I, et al. Naringin prevents cyclophosphamide-induced hepatotoxicity in rats by attenuating oxidative stress,fibrosis,and inflammation[J]. Food and Chemical Toxicology, 2021, 153:112266.

DOI

[15]
EL-DESOKY A H, ABDEL-RAHMAN R F, AHMED O K, et al. Anti-inflammatory and antioxidant activities of naringin isolated from Carissa carandas L.:in vitro and in vivo evidence[J]. Phytomedicine, 2018, 42:126-134.

DOI PMID

[16]
CHEN R C, SUN G B, WANG J, et al. Naringin protects against anoxia/reoxygenation-induced apoptosis in H9C2 cells via the Nrf2 signaling pathway[J]. Food&Function, 2015, 6(4):1331-1344.

[17]
KULASEKARAN G, GANAPASAM S. Neuroprotective efficacy of naringin on 3-nitropropionic acid-induced mitochondrial dysfunction through the modulation of Nrf2 signaling pathway in PC12 cells[J]. Molecular and Cellular Biochemistry, 2015, 409(1/2):199-211.

DOI

[18]
GOPINATH K, SUDHANDIRAN G. Naringin modulates oxidative stress and inflammation in 3-nitropropionic acid-induced neurodegeneration through the activation of nuclear factor-erythroid 2-related factor-2 signalling pathway[J]. Neuroscience, 2012, 227:134-143.

DOI PMID

[19]
WU Q, YU P F, BI Y Z, et al. Naringin regulates mitochondrial dynamics to protect against acetaminophen-induced hepatotoxicity by activating the AMPK/Nrf2 signaling pathway in vitro[J]. Brazilian Journal of Medical and Biological Research, 2022, 55:e12040.

DOI

[20]
GUIHUA X, SHUYIN L, JINLIANG G, et al. Naringin protects ovalbumin-induced airway inflammation in a mouse model of asthma[J]. Inflammation, 2016, 39(2):891-899.

DOI PMID

[21]
ZHANG H H, ZHOU X J, ZHONG Y S, et al. Naringin suppressed airway inflammation and ameliorated pulmonary endothelial hyperpermeability by upregulating aquaporin1 in lipopolysaccharide/cigarette smoke-induced mice[J]. Biomedicine & Pharmacotherapy, 2022, 150:113035.

DOI

[22]
ZHAI X H, DAI T T, CHI Z C, et al. Naringin alleviates acetaminophen-induced acute liver injury by activating Nrf2 via CHAC2 upregulation[J]. Environmental Toxicology, 2022, 37(6):1332-1342.

DOI

[23]
MOHANTY S, KONKIMALLA V B, PAL A, et al. Naringin as sustained delivery nanoparticles ameliorates the anti-inflammatory activity in a freund’s complete adjuvant-induced arthritis model[J]. ACS Omega, 2021, 6(43):28630-28641.

DOI

[24]
CAO R G, WU X, GUO H, et al. Naringin exhibited therapeutic effects against DSS-induced mice ulcerative colitis in intestinal barrier-dependent manner[J]. Molecules, 2021, 26(21):6604.

DOI

[25]
AHMAD S F, ATTIA S M, BAKHEET S A, et al. Naringin attenuates the development of carrageenan-induced acute lung inflammation through inhibition of NF-κb,STAT3 and pro-inflammatory mediators and enhancement of IκBα and anti-inflammatory cytokines[J]. Inflammation, 2015, 38(2):846-857.

DOI

[26]
RI M H, LI M Y, XING Y, et al. Narirutin exerts anti-inflammatory activity by inhibiting NLRP3 inflammasome activation in macrophages[J]. Phytotherapy Research, 2023, 37(4):1293-1308.

DOI PMID

[27]
LIU Y, SU W W, WANG S, et al. Naringin inhibits chemokine production in an LPS-induced raw 264.7 macrophage cell line[J]. Molecular Medicine Reports, 2012, 6(6):1343-1350.

DOI PMID

[28]
KANNO S I, SHOUJI A, TOMIZAWA A, et al. Inhibitory effect of naringin on lipopolysaccharide (LPS)-induced endotoxin shock in mice and nitric oxide production in RAW 264.7 macrophages[J]. Life Sciences, 2006, 78(7):673-681.

DOI

[29]
GHANBARI-MOVAHED M, JACKSON G, FARZAEI M H, et al. A systematic review of the preventive and therapeutic effects of naringin against human malignancies[J]. Frontiers in Pharmacology, 2021, 12:639840.

DOI

[30]
LIN R Y, HU X X, CHEN S R, et al. Naringin induces endoplasmic reticulum stress-mediated apoptosis,inhibits β-catenin pathway and arrests cell cycle in cervical cancer cells[J]. Acta Biochimica Polonica, 2020, 67(2):181-188.

[31]
ZHU L, SHI J, MU M C, et al. Naringin inhibits the proliferation,migration,invasion and epithelial-to-mesenchymal transition of gastric cancer cells via the PI3K/Akt signaling pathway[J]. Alternative Therapies in Health and Medicine, 2023, 29(1):191-197.

[32]
BANJERDPONGCHAI R, WUDTIWAI B, KHAWON P. Induction of human hepatocellular carcinoma HepG2 cell apoptosis by naringin[J]. Asian Pacific Journal of Cancer Prevention, 2016, 17(7):3289-3294.

PMID

[33]
RAMESH E, ALSHATWI A A. Naringin induces death receptor and mitochondria-mediated apoptosis in human cervical cancer (SiHa) cells[J]. Food and Chemical Toxicology, 2013, 51:97-105.

DOI PMID

[34]
XU C X, HUANG X Y, HUANG Y B, et al. Naringin induces apoptosis of gastric carcinoma cells via blocking the PI3K/Akt pathway and activating pro?death autophagy[J]. Molecular Medicine Reports, 2021, 24(5):772.

DOI

[35]
RAHA S, YUMNAM S, HONG G E, et al. Naringin induces autophagy-mediated growth inhibition by downregulating the PI3K/Akt/mTOR cascade via activation of MAPK pathways in AGS cancer cells[J]. International Journal of Oncology, 2015, 47(3):1061-1069.

DOI PMID

[36]
AROUI S, AOUEY B, CHTOUROU Y, et al. Naringin suppresses cell metastasis and the expression of matrix metalloproteinases (MMP-2 and MMP-9) via the inhibition of ERK-P38-JNK signaling pathway in human glioblastoma[J]. Chemico-Biological Interactions, 2016, 244:195-203.

DOI PMID

[37]
AROUI S, FETOUI H, KENANI A. Natural dietary compound naringin inhibits glioblastoma cancer neoangiogenesis[J]. BMC Pharmacology and Toxicology, 2020, 21(1):46.

DOI

[38]
LIU X L, YANG X Y, CHEN F, et al. Combined application of doxorubicin and naringin enhances the antitumor efficiency and attenuates the toxicity of doxorubicin in HeLa cervical cancer cells[J]. International Journal of Clinical and Experimental Pathology, 2017, 10(7):7303-7311.

PMID

[39]
BARBER E, HOUGHTON M J, VISVANATHAN R, et al. Measuring key human carbohydrate digestive enzyme activities using high-performance anion-exchange chromatography with pulsed amperometric detection[J]. Nature Protocols, 2022, 17(12):2882-2919.

DOI

[40]
DENG N, ZHENG B S, LI T, et al. Assessment of the phenolic profiles,hypoglycemic activity,and molecular mechanism of different highland barley (Hordeum vulgare L.) varieties[J]. International Journal of Molecular Sciences, 2020, 21(4):1175.

DOI

[41]
SAHNOUN M, TRABELSI S, BEJAR S. Citrus flavonoids collectively dominate the α-amylase and α-glucosidase inhibitions[J]. Biologia, 2017, 72(7):764-773.

DOI

[42]
JUNG U J, CHOI M S, LEE M K, et al. The hypoglycemic effects of hesperidin and naringin are partly mediated by hepatic glucose-regulating enzymes in C57BL/KsJ-db/db mice[J]. The Journal of Nutrition, 2004, 134(10):2499-2503.

DOI

[43]
JUNG U J, LEE M K, PARK Y B, et al. Effect of citrus flavonoids on lipid metabolism and glucose-regulating enzyme mRNA levels in type-2 diabetic mice[J]. The International Journal of Biochemistry & Cell Biology, 2006, 38(7):1134-1145.

DOI

[44]
BOUCHER J, KLEINRIDDERS A, KAHN C R. Insulin receptor signaling in normal and insulin-resistant states[J]. Cold Spring Harbor Perspectives in Biology, 2014, 6(1):a009191.

DOI

[45]
LIM Y J, KIM J H, PAN J H, et al. Naringin protects pancreatic β-cells against oxidative stress-induced apoptosis by inhibiting both intrinsic and extrinsic pathways in insulin-deficient diabetic mice[J]. Molecular Nutrition Food Research, 2018, 62(5):1700810.

DOI

[46]
SHARMA A K, BHARTI S, OJHA S, et al. Up-regulation of PPARγ,heat shock protein-27 and -72 by naringin attenuates insulin resistance,β-cell dysfunction,hepatic steatosis and kidney damage in a rat model of type 2 diabetes[J]. British Journal of Nutrition, 2011, 106(11):1713-1723.

DOI

[47]
TERMKWANCHAROEN C, MALAKUL W, PHETRUNGNAPHA A, et al. Naringin ameliorates skeletal muscle atrophy and improves insulin resistance in high-fat-diet-induced insulin resistance in obese rats[J]. Nutrients, 2022, 14(19):4120.

DOI

[48]
BATCHULUUN B, PINKOSKY S L, STEINBERG G R. Lipogenesis inhibitors:therapeutic opportunities and challenges[J]. Nature Reviews Drug Discovery, 2022, 21(4):283-305.

DOI

[49]
GLUCHOWSKI N L, GABRIEL K R, CHITRAJU C, et al. Hepatocyte deletion of triglyceride-synthesis enzyme acyl CoA:diacylglycerol acyltransferase 2 reduces steatosis without increasing inflammation or fibrosis in mice[J]. Hepatology, 2019, 70(6):1972-1985.

DOI

[50]
KARASAWA K, TANIGAWA K, HARADA A, et al. Transcriptional regulation of acyl-CoA:glycerol-sn-3-phosphate acyltransferases[J]. International Journal of Molecular Sciences, 2019, 20(4):964.

DOI

[51]
PENGNET S, SUMARITHUM P, PHONGNU N, et al. Naringin attenuates fructose-induced nafld progression in rats through reducing endogenous triglyceride synthesis and activating the Nrf2/HO-1 pathway[J]. Frontiers in Pharmacology, 2022, 13:1049818.

DOI

[52]
熊朝栋, 陈红, 陈丹, 等. 玳玳果黄酮提取物关键效应组分辨识及调控脂质代谢作用机制研究[J]. 中国现代应用药学, 2022, 39(14):1818-1827.

XIONG C D, CHEN H, CHEN D, et al. Study on the identification of the key effect components and the lipid metabolism mechanism for Daidai flavonoid extracts[J]. Chinese Journal of Modern Applied Pharmacy, 2022, 39(14):1818-1827. (in Chinese)

[53]
ZHANG X H, ZHANG Y Z, GAO W, et al. Naringin improves lipid metabolism in a tissue-engineered liver model of NAFLD and the underlying mechanisms[J]. Life Sciences, 2021, 277:119487.

DOI

[54]
JEON S M. Regulation and function of AMPK in physiology and diseases[J]. Experimental and Molecular Medicine, 2016, 48(7):e245.

DOI

[55]
TIAN X, RU Q, XIONG Q, et al. Catalpol attenuates hepatic steatosis by regulating lipid metabolism via AMP-activated protein kinase activation[J]. BioMed Research International, 2020, 2020:6708061.

[56]
DAYARATHNE L A, RANAWEERA S S, NATRAJ P, et al. Restoration of the adipogenic gene expression by naringenin and naringin in 3T3-L1 adipocytes[J]. Journal of Veterinary Science, 2021, 22(4):e55.

DOI PMID

[57]
JIANG X, LI A Y, WANG Y P, et al. Ameliorative effect of naringin against thiram-induced tibial dyschondroplasia in broiler chicken[J]. Environmental Science and Pollution Research, 2020, 27(10):11337-11348.

DOI

[58]
EBIRIM C G, ESAN O, ADETONA M O, et al. Naringin administration mitigates oxidative stress,anemia,and hypertension in lead acetate-induced cardio-renal dysfunction in cockerel chicks[J]. Environmental Science and Pollution Research International, 2023, 30(12):34890-34903.

DOI

[59]
RANJBAR Z, TORKI M, KARIMI TORSHIZI A A. In ovo injection of flavanone on bone quality characteristics,biochemical parameters and antioxidant enzyme status of blood in daily chicks[J]. Journal of Animal Physiology and Animal Nutrition, 2019, 103(5):1418-1426.

DOI

[60]
GOLIOMYTIS M, KARTSONAS N, CHARISMIADOU M A, et al. The influence of naringin or hesperidin dietary supplementation on broiler meat quality and oxidative stability[J]. PLoS One, 2015, 10(10):e0141652.

DOI

[61]
LI H, HOU Y Y, HU J N, et al. Dietary naringin supplementation on hepatic yolk precursors formation and antioxidant capacity of three-yellow breeder hens during the late laying period[J]. Poultry Science, 2023, 102(5):102605.

DOI

[62]
LI H, HOU Y Y, CHEN J M, et al. Dietary naringin supplementation on laying performance and antioxidant capacity of three-yellow breeder hens during the late laying period[J]. Poultry Science, 2022, 101(9):102023.

DOI

[63]
BAO T T, YAO J W, ZHOU S, et al. Naringin prevents follicular atresia by inhibiting oxidative stress in the aging chicken[J]. Poultry Science, 2022, 101(7):101891.

DOI

[64]
HAGER-THEODORIDES A L, MASSOURAS T, SIMITZIS P E, et al. Hesperidin and naringin improve broiler meat fatty acid profile and modulate the expression of genes involved in fatty acid β-oxidation and antioxidant defense in a dose dependent manner[J]. Foods, 2021, 10(4):739.

DOI

[65]
GOLIOMYTIS M, SIMITZIS P, PAPALEXI A, et al. Influence of citrus flavonoids on laying hen performance,inflammatory immune response,egg quality and yolk oxidative stability[J]. British Poultry Science, 2019, 60(3):272-278.

DOI

[66]
GOODARZI BOROOJENI F, MÄNNER K, ZENTEK J. The impacts of Macleaya cordata extract and naringin inclusion in post-weaning piglet diets on performance,nutrient digestibility and intestinal histomorphology[J]. Archives of Animal Nutrition, 2018, 72(3):178-189.

DOI

[67]
WANG Q, WANG J, QI R L, et al. Naringin supplementation affects performance,carcass traits,meat quality and oxidative stability of finishing pigs[J]. South African Journal of Animal Science, 2020, 50(1):78-87.

DOI

[68]
李赤翎, 俞建, 曾亮, 等. 柚皮苷对猪肉的抗氧化作用的研究[J]. 食品研究与开发, 2008, 29(10):20-23.

LI C L, YU J, ZENG L, et al. Study of antioxid ation of naringin on pork meat[J]. Food Research and Development, 2008, 29(10):20-23. (in Chinese)

[69]
SUN H, ZHAO F F, HOU F Y, et al. Influences of naringin supplementation on ruminal fermentation,inflammatory response,antioxidant capacity and bacterial community in high-concentrate diet of fattening goats[J]. Italian Journal of Animal Science, 2022, 21(1):1498-1507.

DOI

[70]
BALCELLS J, ARIS A, SERRANO A, et al. Effects of an extract of plant flavonoids (Bioflavex) on rumen fermentation and performance in heifers fed high-concentrate diets[J]. Journal of Animal Science, 2012, 90(13):4975-4984.

DOI PMID

[71]
SHI L L, XU Y Q, MAO C Y, et al. Effects of heat stress on antioxidant status and immune function and expression of related genes in lambs[J]. International Journal of Biometeorology, 2020, 64(12):2093-2104.

DOI

[72]
REITH R R, SIECK R L, GRIJALVA P C, et al. Transcriptome analyses indicate that heat stress-induced inflammation in white adipose tissue and oxidative stress in skeletal muscle is partially moderated by zilpaterol supplementation in beef cattle[J]. Journal of Animal Science, 2022, 100(3):skac019.

DOI

[73]
ALHIDARY I A, ABDELRAHMAN M M. Effects of naringin supplementation on productive performance,antioxidant status and immune response in heat-stressed lambs[J]. Small Ruminant Research, 2016, 138:31-36.

DOI

[74]
SIMITZIS P E, CHARISMIADOU M A, GOLIOMYTIS M, et al. Antioxidant status,meat oxidative stability and quality characteristics of lambs fed with hesperidin,naringin or α-tocopheryl acetate supplemented diets[J]. Journal of the Science of Food and Agriculture, 2019, 99(1):343-349.

DOI

[75]
SIMITZIS P, MASSOURAS T, GOLIOMYTIS M, et al. The effects of hesperidin or naringin dietary supplementation on the milk properties of dairy ewes[J]. Journal of the Science of Food and Agriculture, 2019, 99(14):6515-6521.

DOI PMID

文章导航

/