研究论文

单宁和裂壶藻粉对滩羊生长性能及瘤胃菌群多样性的影响

  • 温红瑞 , 1 ,
  • 高昌鹏 1 ,
  • 杨万彪 1 ,
  • 刘文茂 2 ,
  • 周玉香 , 1, *
展开
  • 1 宁夏大学农学院,银川 750021
  • 2 宁夏中宁文茂生态饲料有限公司,中宁 755100
*周玉香,教授,博士生导师,E-mail:

温红瑞(1998—),女,河北张家口人,硕士研究生,从事反刍动物营养与饲料研究。E-mail:

Office editor: 陈鑫

收稿日期: 2023-05-03

  网络出版日期: 2023-10-12

基金资助

宁夏科技厅重点研发项目(2021BEF02027)

Effects of Tannin and Schizochytrium Powder on Growth Performance and Rumen Microflora Diversity of Tan Sheep

  • WEN Hongrui , 1 ,
  • GAO Changpeng 1 ,
  • YANG Wanbiao 1 ,
  • LIU Wenmao 2 ,
  • ZHOU Yuxiang , 1, *
Expand
  • 1 College of Agriculture, Ningxia University, Yinchuan 750021, China
  • 2 Zhongning Wenmao Ecological Feed Limited Liability Company of Ningxia, Zhongning 755100, China
*professor, E-mail:

Received date: 2023-05-03

  Online published: 2023-10-12

摘要

本试验旨在探究饲粮中添加单宁和裂壶藻粉对滩羊生长性能及瘤胃菌群多样性的影响。选取体重[(25.53±3.18) kg]相近的5月龄健康滩羊公羔48只,随机均分为4组,每组12个重复,对照组饲喂基础饲粮,试验Ⅰ组饲喂基础饲粮+0.4%单宁,试验Ⅱ组饲喂基础饲粮+2.0%裂壶藻粉,试验Ⅲ组饲喂基础饲粮+0.4%单宁+2.0%裂壶藻粉。试验期共105 d,其中预试期15 d,正试期90 d。结果表明:1)与对照组相比,试验Ⅰ组羊只的总增重显著增加(P<0.05)。2)各试验组的操作分类单元数目均低于对照组,表现为对照组>试验Ⅰ组>试验Ⅱ组>试验Ⅲ组。3)与对照组相比,试验Ⅲ组Sobs指数、Ace指数和Chao1指数均出现显著下降(P<0.05),与试验Ⅰ组相比,试验Ⅲ组Ace指数和Chao1指数也出现了显著下降(P<0.05)。4)在门水平上,对照组、试验Ⅰ组和试验Ⅱ组的优势菌门均为拟杆菌门和厚壁菌门,试验Ⅲ组的优势菌门为拟杆菌门、厚壁菌门和变形菌门。与对照组相比,各试验组脱硫菌门、Patescibacteria的相对丰度出现显著变化(P<0.05),浮霉菌门的相对丰度出现极显著变化(P<0.01)。5)在属水平上,普雷沃氏菌属和理研菌科_RC9_肠道群为优势菌属。与对照组相比,各试验组未排位拟杆菌目_BS11_肠道群、理研菌科_RC9_肠道群、未排位拟杆菌目_RF16_群、norank_Muribaculaceae和韦荣氏球菌科_UCG-001的相对丰度出现显著变化(P<0.05),脱硫弧菌属的相对丰度出现极显著变化(P<0.01)。6)与试验Ⅰ组相比,试验Ⅱ组的滩羊瘤胃菌群的氨基酸代谢功能通路相对丰度显著降低(P<0.05)。综上所述,饲粮中添加单宁和裂壶藻粉均会影响滩羊生长性能及瘤胃微生物菌群结构,促进部分有益菌的增殖,并改善代谢功能;并且,以单独添加0.4%单宁的效果最好,同时添加0.4%单宁和2.0%裂壶藻粉效果次之,单独添加2.0%裂壶藻粉效果不明显。

本文引用格式

温红瑞 , 高昌鹏 , 杨万彪 , 刘文茂 , 周玉香 . 单宁和裂壶藻粉对滩羊生长性能及瘤胃菌群多样性的影响[J]. 动物营养学报, 2023 , 35(10) : 6546 -6559 . DOI: 10.12418/CJAN2023.599

Abstract

This experiment was conducted to investigate the effects of dietary tannin and Schizochytrium powder on growth performance and rumen microflora diversity of Tan sheep. Forty-eight healthy Tan sheep male lambs with similar body weight [(25.53±3.18) kg] were randomly divided into 4 groups with 12 lambs in each group. The control group was fed a basal diet, trial group Ⅰ was fed the basal diet+0.4% tannin, trial group Ⅱ was fed the basal diet+2.0% Schizochytrium powder, and trial group Ⅲ was fed the basal diet+0.4% tannin+2.0% Schizochytrium powder. The test period was 105 days. The pre-feeding period lasted for 15 days and the normal feeding period lasted for 90 days. The results showed as follows: 1) compared with the control group, the total weight gain of sheep in trial group Ⅰ was significantly increased (P>0.05). 2) The number of operational taxonomic units (OTUs) in experimental groups was lower than that in control group, which was as follows: control group > trial group Ⅰ > trial group Ⅱ > trial group Ⅲ. 3) Compared with the control group, Sobs index, Ace index and Chao1 index in trial group Ⅲ were significantly decreased (P<0.05), and compared with trial group Ⅰ, Ace index and Chao1 index in trial group Ⅲ were also significantly decreased (P<0.05). 4) At the phylum level, Bacteroidetes and Firmicutes were dominant in control group, trial groups Ⅰ and Ⅱ, and Bacteroidetes, Firmicutes and Proteobacteria were dominant in trial group Ⅲ. Compared with the control group, the relative abundance of Desulfobacterota and Patescibacteria in trial groups changed significantly (P<0.05) and the relative abundance of Planctomycetota in trial groups changed extremely significantly(P<0.01). 5) At the genus level, Prevotella and Rikenellaceae_RC9_gut_group were the dominant genus. Compared with the control group, the relative abundance of norank_Bacteroidales_BS11_gut_group, Rikenellaceae_RC9_gut_group, norank_Bacteroidales_RF16_group, norank_Muribacula ceae, Veillonellaceae_UCG-001 in trial groups were significantly changed (P<0.05), and the relative abundance of Desulfovibrio in trial groups changed extremely significantly(P<0.01). 6) Compared with trial group Ⅰ, the relative abundance of amino acid metabolic functional pathway of rumen flora of Tan sheep in trial group Ⅱ was significantly decreased (P<0.05). It is concluded that dietary supplementation of tannin and Schizochytrium powder can affect the growth performance and rumen microflora structure of Tan sheep, promote the proliferation of some beneficial bacteria, and improve metabolic function,and the best effect is the addition of 0.4% tannin alone, followed by the addition of 0.4% tannin and 2.0% Schizochytrium powder, and effect is not obvious by adding 2.0% Schizochytrium powder alone.

绿色发展背景下,饲料行业迈入“无抗”时代。但在畜牧生产过程中,细菌性和病毒性等疾病频发、动物机体生长缓慢、发病率高等问题成为制约我国畜牧业发展的瓶颈。因而寻找替抗饲料添加剂迫在眉睫。
单宁作为一种天然植物多酚,具有较强的收敛性和生物学活性,如抗氧化[1]、抗菌[2]、抗炎[3]、抗病毒[4]等。研究表明,添加适量的单宁可以调节瘤胃微生物区系[5]、增加“瘤胃逃逸蛋白”的数量[6]、提高蛋白质利用率,并且单宁也是潜在的生物加氢调节剂,它可以通过调控多不饱和脂肪酸(PUFAs)的合成来改善肉品质[7],对反刍动物生长有着积极影响。但添加过量的单宁也会对动物产生副作用[8]
裂壶藻,又称裂殖壶藻,是从海水中分离筛选到的单细胞微藻,其增殖速度快、发酵周期短。在生长过程中积累了大量的营养物质和对动物有益的活性成分,如n-3PUFAs、蛋白质、虾青素和类胡萝卜素等,可作为一种功能性添加剂或代替部分蛋白质源和油脂使用。添加适量的裂壶藻粉可以增加PUFAs的含量,从而促进脂质代谢[9],改善肉品质[10],提高免疫性能[11]
本课题组前期研究表明,单独添加0.4%单宁或2.0%裂壶藻粉均对滩羊有促生长、提高免疫力、改善肉品质的作用[12-13]。但两者组合添加对滩羊瘤胃菌群结构的影响鲜见报道。且单宁和PUFAs在反刍动物上的研究,也只是集中于缩合单宁和亚油酸(LA)或亚麻酸(LNA)对其生产性能表型指标的影响[14-15]。因此,本试验在课题组前期试验的基础上,研究饲粮中添加0.4%单宁+2.0%裂壶藻粉对滩羊生长性能及其瘤胃菌群结构的影响,以期为单宁和裂壶藻粉在滩羊生产实践中的应用提供理论依据。

1 材料与方法

1.1 试验设计

试验于2022年7月至2022年11月在中宁县文茂草源生态饲料有限公司进行。试验采用单因素随机试验设计,选取体重[(25.53±3.18) kg]相近的5月龄健康滩羊公羔48只,随机均分为4组,每组12个重复。对照组饲喂基础饲粮,试验Ⅰ组饲喂基础饲粮+0.4%单宁(水解单宁含量为76%),试验Ⅱ组饲喂基础饲粮+2.0%裂壶藻粉(干物质含量96%,粗蛋白质含量26%,粗脂肪含量40%,二十二碳六烯酸含量15%)、试验Ⅲ组饲喂基础饲粮+0.4%单宁+2.0%裂壶藻粉。试验期共105 d,其中预试期15 d,正试期90 d。

1.2 试验饲粮

试验饲粮按照《肉羊饲养标准》(NY/T 816—2021)并结合实际生产进行配制,由于裂壶藻粉中含有大量的营养物质,而单宁中营养物质较少,因而选择用裂壶藻粉代替玉米,单宁代替小苏打。各组饲粮营养水平相近,精粗比为45∶55。试验饲粮组成及营养水平见表1
表1 试验饲粮组成及营养水平(干物质基础)

Table 1 Composition and nutrient levels of trial diets (DM basis)%

项目
Items
对照组
Control group
试验Ⅰ组
Trial group Ⅰ
试验Ⅱ组
Trial group Ⅱ
试验Ⅲ组
Trial group Ⅲ
原料 Ingredients
苜蓿干草 Alfalfa hay 36.00 36.00 36.00 36.00
玉米秸秆 Corn stalk 14.00 14.00 14.00 14.00
玉米 Corn 29.80 29.80 27.80 27.80
豆粕 Soybean meal 6.00 6.00 6.00 6.00
麸皮 Wheat bran 3.00 3.00 3.00 3.00
玉米干酒糟及其可溶物 Corn DDGS 8.00 8.00 8.00 8.00
食盐 NaCl 0.90 0.90 0.90 0.90
石粉 Limestone 0.30 0.30 0.30 0.30
预混料 Premix1) 1.00 1.00 1.00 1.00
小苏打 NaHCO3 1.00 0.60 1.00 0.60
栗木单宁 Chestnut tannin 0.40 0.40
裂壶藻粉 Schizochytrium powder 2.00 2.00
合计 Total 100.00 100.00 100.00 100.00
营养水平 Nutrient levels2)
代谢能 ME/(MJ/kg) 10.88 10.88 10.61 10.61
粗蛋白质 CP 15.39 15.39 15.75 15.75
钙 Ca 0.88 0.88 0.88 0.88
磷 P 0.34 0.34 0.33 0.33
中性洗涤纤维 NDF 37.04 37.04 36.85 36.85
酸性洗涤纤维 ADF 22.56 22.56 22.50 22.50

1)每千克预混料含有 One kg of premix contented the following:VA 224 000 IU,VD3 100 000 IU,VE 700 mg,Mn 1 200 mg,Se 4.50 mg,Zn 1 900 mg,NaCl 160 mg,Ca 200 mg,P 40 mg。

2)代谢能为计算值,其余为实测值。ME was a calculated value, while the others were measured values.

1.3 饲养管理

在试验开始前,对羊圈进行打扫、消毒处理,并对试验羊进行统一编号、布病检测和驱虫防疫。所有试验羊每天分2次(07:00和17:00)饲喂全混合日粮,期间保障试验羊自由采食和自由饮水,每天定时清理料槽,记录投料量和剩料量,用于计算干物质采食量(DMI)。试验羊在正试期开始和结束时空腹称重、记录,并计算总增重(TG)、平均日增重(ADG)和料重比(F/G)。

1.4 瘤胃液的采集和处理

在正试期第90天,晨饲前每组随机选择6只羊,用口腔瘤胃液采集器采集瘤胃液50 mL,分装于2 mL冻存管中,置于-80 ℃保存,用于后续瘤胃微生物多样性分析。

1.5 测序及生物信息学分析

提取样品总DNA、构建文库及测序由上海美吉生物医药科技有限公司完成,采用Illumina Miseq平台测序。测序得到的原始数据经质控优化得到有效数据,然后进行物种注释分析、物种差异比较分析。

1.6 数据处理与分析

生长性能数据通过Excel 2010初步整理后,采用SPSS 27.0统计软件进行单因素方差分析,LSD多重比较法进行组间比较。微生物数据通过美吉生物云平台进行分析,使用非参数Kruskal-Wallis秩和检验分析瘤胃液菌群多样性指数组间差异和微生物门、属水平相对丰度的变化,运用PICRUSt2预测菌群基因组功能与KEGG数据库对比,进行菌群代谢功能的预测。利用R语言工具(version 3.3.1)作图。结果均以图或表的形式列出,表中数据用平均值±均值标准误表示。P<0.05表示差异显著,P<0.01表示差异极显著,P>0.05表示差异不显著。

2 结果与分析

2.1 单宁和裂壶藻粉对滩羊生长性能的影响

表2可知,各组羊只的初始体重和终末体重均无显著差异(P>0.05)。与对照组相比,各试验组羊只的总增重和平均日增重都有所提高,其中试验Ⅰ组羊只的总增重显著增加(P<0.05)。与对照组相比,试验Ⅰ组羊只的总增重和平均日增重分别增加了22.64%和16.15%;试验Ⅱ组羊只的总增重和平均日增重分别增加了14.54%和8.76%;试验Ⅲ组羊只的总增重和平均日增重分别增加了15.43%和9.58%。各试验组羊只的干物质采食量和料重比均低于对照组,但差异不显著(P>0.05)。
表2 单宁和裂壶藻粉对滩羊生长性能的影响

Table 2 Effects of tannin and Schizochytrium powder on growth performance of Tan sheep

项目
Items
对照组
Control group
试验Ⅰ组
Trial groupⅠ
试验Ⅱ组
Trial group Ⅱ
试验Ⅲ组
Trial groupⅢ
P
P-value
初始体重 IBW/kg 25.04±3.87 25.39±3.42 25.06±2.59 25.30±2.86 0.995
终末体重 FBW/kg 34.05±3.81 36.44±2.38 35.38±1.67 35.39±3.56 0.456
总增重 TG/kg 9.01±1.42a 11.05±2.10b 10.32±1.64ab 10.40±1.43ab 0.021
平均日增重 ADG/(g/d) 105.41±12.25 122.43±23.48 114.64±18.27 115.51±18.14 0.324
干物质采食量DMI/(g/d) 1 104.32±76.68 1 101.00±75.23 1 094.11±75.89 1 099.31±74.84 0.814
料重比 F/G 10.61±1.37 9.27±1.68 9.77±1.67 9.68±1.39 0.378

同行数据肩标不同小写字母表示差异显著(P<0.05),不同大写字母表示差异极显著(P<0.01),无字母或相同字母表示差异不显著(P>0.05)。下表同。

In the same row, values with different small letter superscripts mean significant difference (P<0.05), with different capital letter superscripts mean significant difference (P<0.01), while with no letter or the same letter superscripts mean no significant difference (P>0.05). The same as below.

2.2 单宁和裂壶藻粉对滩羊瘤胃菌群结构的影响

2.2.1 操作分类单元(OTUs)聚类分析
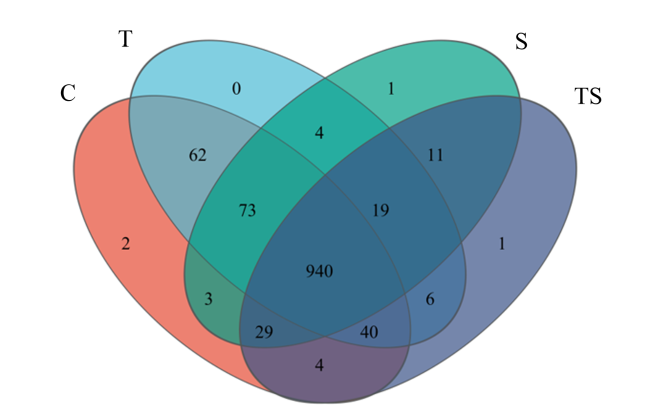
经Illumina Miseq测序结束后,除去低质量序列,通过序列拼接,应用Mouthur,根据相似度97%的原则,进行OTUs划分。根据OTUs聚类分析结果,分析24个样品中OTUs的分布,并绘制韦恩图(图1)。由图1可知,对照组中发现1 153个OTUs,试验Ⅰ组中发现1 144个OTUs,试验Ⅱ组中发现1 080个OTUs,试验Ⅲ组中发现1 050个OTUs,共享了940个OTUs,表明添加单宁、裂壶藻粉会降低滩羊瘤胃液中OTUs数目,即降低细菌菌群的种类。
图1 瘤胃菌群韦恩图

C:对照组;T:试验Ⅰ组;S:试验Ⅱ组;TS:试验Ⅲ组。下图同。

Fig.1 Venn graph of microflora in rumen

C: control group; T: trial groupⅠ; S: trial groupⅡ; TS: trial group Ⅲ. The same as below.

2.2.2 Alpha多样性分析

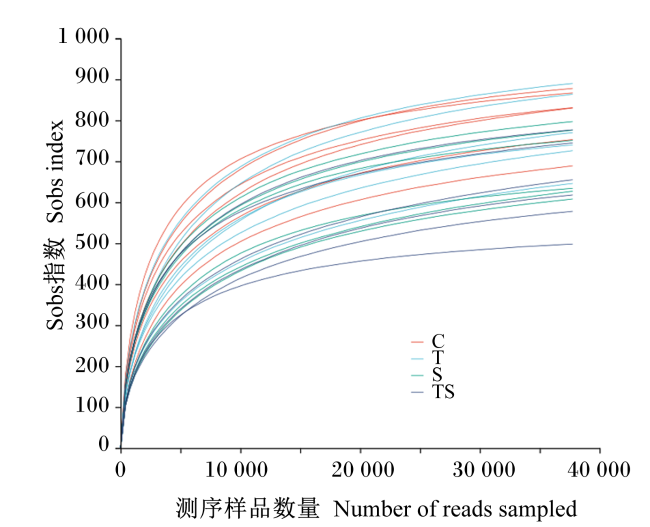
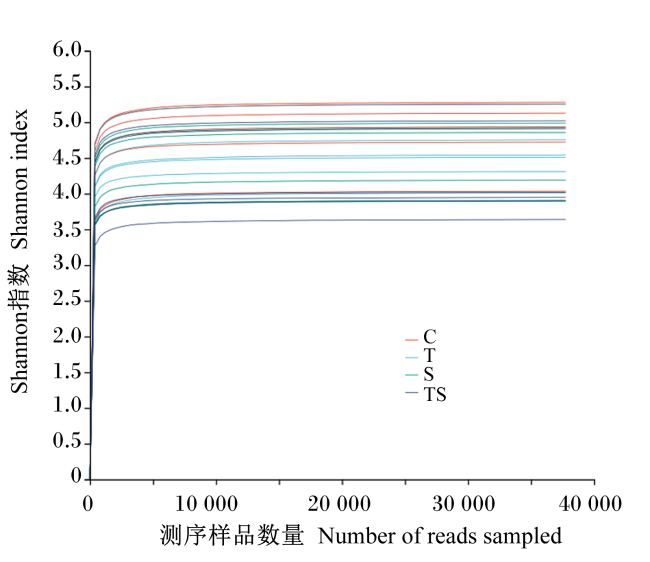
图2可知,所有样品的Sobs指数稀释曲线均为先陡然升高,后趋于平缓,表明测序数据量渐近合理,更深入的测序对滩羊瘤胃液中检测出新的OTUs贡献很小。由图3可知,各样品Shannon指数稀释曲线均为先直线上升,后骤然到达平台期,表明测序趋向饱和,即测序深度已覆盖样品中绝大多数微生物生物种类,能够进行细菌多样性分析。
图2 样品的Sobs指数稀释曲线

Fig.2 Sobs index dilution curve of samples

图3 样品的Shannon指数曲线

Fig.3 Shannon index curve of samples

2.2.3 微生物群落Alpha多样性分析

表3可知,各组间Shannon指数和Simpson指数均差异不显著(P>0.05),表明无论是单独添加单宁或裂壶藻粉还是同时添加,均不会对滩羊瘤胃菌群多样性产生影响。但与对照组相比,试验Ⅲ组Sobs指数、Ace指数和Chao1指数均出现显著下降(P<0.05),表明在饲粮中同时添加单宁和裂壶藻粉会降低滩羊瘤胃细菌菌群的种类。与试验Ⅰ组相比,试验Ⅲ组Ace指数和Chao1指数也出现了显著下降(P<0.05),表明在饲粮中同时添加单宁和裂壶藻粉会降低滩羊瘤胃细菌菌群的种类的结果中裂壶藻粉起到了重要的作用。在本试验中,各组覆盖率均大于0.99,说明样品采集足以反映滩羊瘤胃菌群情况。
表3 Alpha多样性

Table 3 Alpha diversity

项目
Items
对照组
Control group
试验Ⅰ组
Trial groupⅠ
试验Ⅱ组
Trial group Ⅱ
试验Ⅲ组
Trial groupⅢ
P
P-value
Sobs指数 Sobs index 808.00±72.91a 772.70±91.00ab 698.80±84.77ab 645.20±104.30b 0.049 6
Shannon指数 Shannon index 4.89±0.47 4.56±0.42 4.46±0.52 4.24±0.58 0.135 9
Simpson指数 Simpson index 0.02±0.02 0.04±0.03 0.04±0.03 0.07±0.05 0.222 6
Ace指数 Ace index 870.30±60.54a 851.00±79.39a 763.30±76.92ab 712.50±115.10b 0.035 4
Chao1指数 Chao1 index 833.20±52.40a 864.80±85.97a 772.30±80.21ab 719.30±118.20b 0.020 5
覆盖率 Coverage 0.997 1±0.000 4 0.996 7±0.000 4 0.997 2±0.000 4 0.997 3±0.000 7 0.240 9

2.2.4 瘤胃菌群主坐标分析(PCoA)

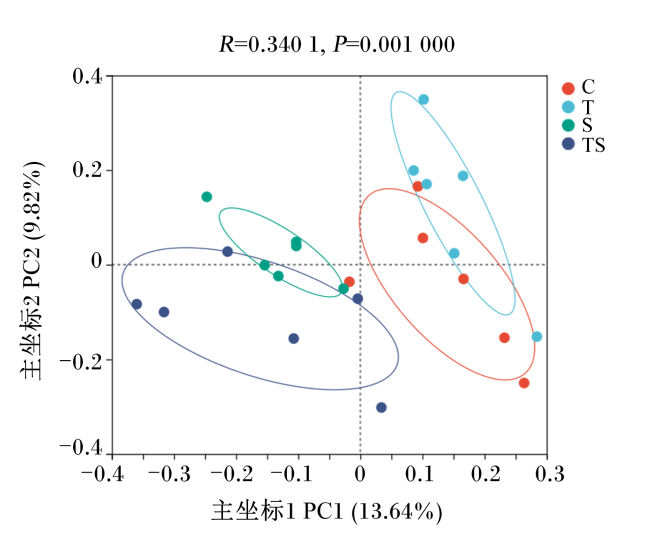
图4可知,对照组与试验Ⅰ组之间的距离比较相近,试验Ⅱ组与试验Ⅲ组的距离较近,而对照组、试验Ⅰ组和试验Ⅱ组、试验Ⅲ组之间的距离比较远,说明对照组与试验Ⅰ组的瘤胃菌群结构相似,试验Ⅱ组与试验Ⅲ组的瘤胃菌群结构相似,而对照组与试验Ⅰ组和试验Ⅱ组、试验Ⅲ组的瘤胃菌群结构存在着差异(P<0.05),也进一步可以说明裂壶藻粉的添加在改变滩羊瘤胃菌群结构中起着重要的作用。
图4 主坐标分析

Fig.4 PCoA

2.2.5 细菌组成与菌群结构分析

2.2.5.1 门水平结构分析

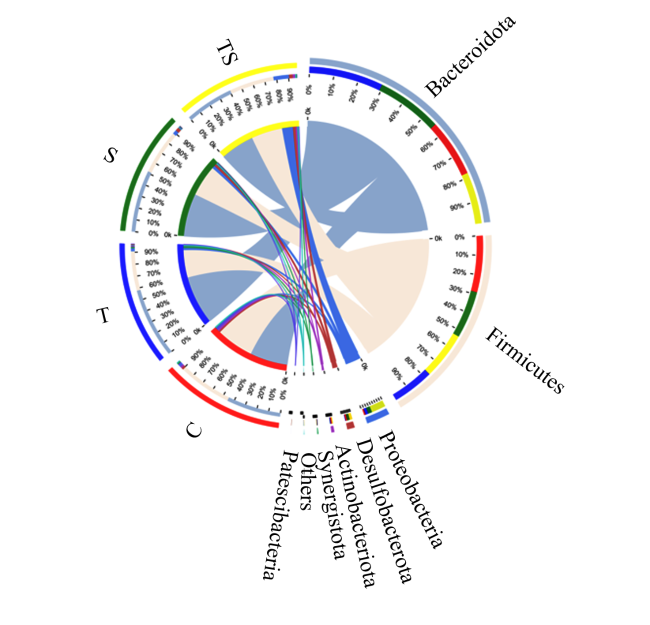
根据物种注释结果,滩羊瘤胃液细菌在门水平上的菌落组成和相对丰度见表4图5,共检测到了16个菌门,包括拟杆菌门(Bacteroidota)、厚壁菌门(Firmicutes)、变形菌门(Proteobacteria)、脱硫菌门(Desulfobacterota)、放线菌门(Actinobacteriota)、互养菌门(Synergistota)、Patescibacteria、疣微菌门(Verrucomicrobiota)、螺旋菌门(Spirochaetota)、未分类菌门(unclassified_k_norank_d_bacteria)、蓝藻门(Cyanobacteria)、浮霉菌门(Planctomycetota)、绿屈挠菌门(Chloroflexi)、丝状杆菌门(Fibrobacterota)、WPS-2、Elusimicrobiota。对照组、试验Ⅰ组和试验Ⅱ组滩羊瘤胃液中的优势菌门均为拟杆菌门和厚壁菌门,占到总细菌数的91.19%以上。试验Ⅲ组的优势菌门为拟杆菌门、厚壁菌门和变形菌门,其中拟杆菌门和厚壁菌门占总细菌数的79.75%,变形菌门占总细菌数的13.21%。与对照组相比,试验Ⅰ组脱硫菌门的相对丰度极显著降低(P<0.01);试验Ⅲ组脱硫菌门的相对丰度显著升高(P<0.05),Patescibacteria的相对丰度显著降低(P<0.05)。与试验Ⅰ组相比,试验Ⅱ组浮霉菌门的相对丰度极显著升高(P<0.01);试验Ⅲ组脱硫菌门的相对丰度显著升高(P<0.05)。
表4 单宁和裂壶藻粉对滩羊瘤胃菌群在门水平上相对丰度的影响

Table 4 Effects of tannin and Schizochytrium powder on rumen microflora relative abundance at phylum level of Tan sheep%

项目
Items
对照组
Control group
试验Ⅰ组
Trial groupⅠ
试验Ⅱ组
Trial group Ⅱ
试验Ⅲ组
Trial groupⅢ
P
P-value
拟杆菌门 Bacteroidota 46.47±17.30 59.84±17.62 52.93±9.37 41.63±15.81 0.213 5
厚壁菌门 Firmicutes 45.73±14.62 33.62±16.29 38.26±10.59 38.12±14.46 0.535 9
变形菌门 Proteobacteria 1.36±1.71 2.53±2.38 3.54±4.79 13.21±18.64 0.358 0
脱硫菌门 Desulfobacterota 1.73±0.73Aa 0.57±0.30Ba 2.98±2.49ABab 3.21±1.98ABb 0.005 5
放线菌门 Actinobacteriota 1.66±1.41 1.08±0.94 0.33±0.29 2.01±3.51 0.138 2
互养菌门 Synergistota 1.10±2.03 1.25±2.71 0.61±0.64 0.58±0.38 0.434 6
Patescibacteria 1.12±0.57a 0.54±0.30ab 0.62±0.33ab 0.30±0.30b 0.017 6
疣微菌门Verrucomicrobiota 0.17±0.13 0.21±0.12 0.22±0.17 0.46±0.26 0.120 3
螺旋菌门 Spirochaetota 0.34±0.24 0.14±0.08 0.16±0.10 0.23±0.31 0.338 5
未分类菌门
Unclassified_k_norank_d_bacteria
0.23±0.35 0.07±0.04 0.17±0.16 0.12±0.10 0.582 1
蓝藻门 Cyanobacteria 0.04±0.04 0.14±0.18 0.13±0.15 0.06±0.04 0.396 8
浮霉菌门 Planctomycetota 0.01±0.01ABab 0.00±0.00Aa 0.02±0.01Bb 0.03±0.04ABab 0.006 6
绿屈挠菌门 Chloroflexi 0.01±0.01 0.00±0.00 0.02±0.02 0.02±0.04 0.787 7
丝状杆菌门 Fibrobacterota 0.01±0.01 0.02±0.02 0.01±0.01 0.00±0.00 0.092 6
WPS-2 0.01±0.01 0.00±0.00 0.01±0.01 0.01±0.01 0.117 2
Elusimicrobiota 0.01±0.02 0.00±0.00 0.01±0.01 0.00±0.00 0.559 7
图5 门水平上瘤胃菌群Circos图

Bacteroidota:拟杆菌门; Firmicutes:厚壁菌门; Proteobacteria:变形菌门;Desulfobacterota:脱硫菌门; Actinobacteriota:放线菌门; Synergistota:互养菌门;Others:其他。

Fig.5 Circos diagram of rumen microflora at phylum level

2.2.5.2 属水平结构分析

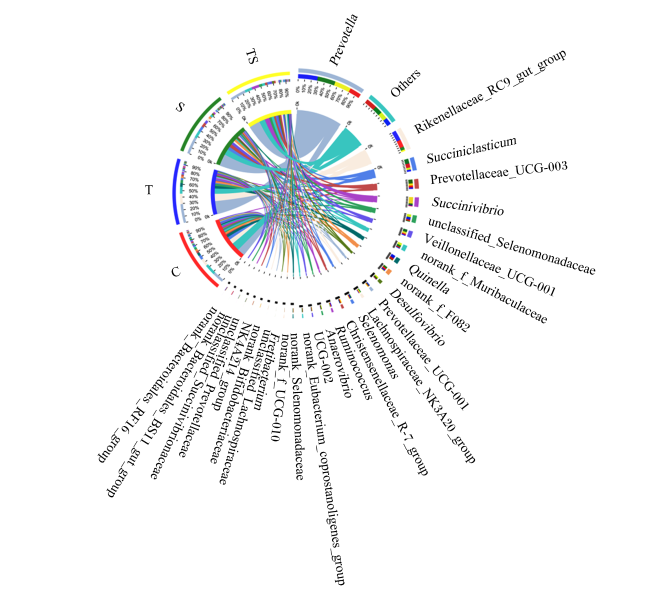
根据物种注释结果,滩羊瘤胃液细菌在属水平上的菌落组成和相对丰度见表5图6。共检测到了175个菌属,其中有29个菌属相对丰度比例在1%以上,分别为普雷沃氏菌属(Prevotella)、理研菌科_RC9_肠道群(Rikenellaceae_RC9_gut_group)、解琥珀酸菌属(Succiniclasticum)、普雷沃氏菌科UCG-003(Prevotellaceae_UCG-003)、琥珀酸弧菌属(Succinivibrio)、未分类硒藻科(unclassified_Selenomonadaceae)、韦荣氏球菌科_UCG-001(Veillonellaceae_UCG-001)、norank_Muribaculaceae、奎因氏菌属(Quinella)、norank_F082、脱硫弧菌属(Desulfovibrio)、普雷沃氏菌科UCG-001(Prevotellaceae_UCG-001)、毛螺菌科_NK3A20_群(Lachnospiraceae_NK3A20_group)、月形单胞菌属(Selenomonas)、克里斯滕森菌科R-7群Christensenellaceae_R-7_group)、瘤胃球菌属(Ruminococcus)等。与对照组相比,试验Ⅰ组脱硫弧菌属的相对丰度极显著降低(P<0.01),未排位拟杆菌目_BS11_肠道群(norank_Bacteroidales_BS11_gut_group)的相对丰度显著降低(P<0.05);试验Ⅱ组理研菌科_RC9_肠道群、未排位拟杆菌目_BS11_肠道群的相对丰度极显著降低(P<0.01);试验Ⅲ组理研菌科_RC9_肠道群、未排位拟杆菌目_BS11_肠道群和未排位拟杆菌目_RF16_群(norank_Bacteroidales_RF16_group)的相对丰度极显著降低(P<0.01)。与试验Ⅰ组相比,试验Ⅱ组norank_Muribaculaceae的相对丰度显著升高(P<0.05);试验Ⅲ组理研菌科_RC9_肠道群和未排位拟杆菌目_RF16_群的相对丰度极显著降低(P<0.01),韦荣氏球菌科_UCG-001的相对丰度显著升高(P<0.05),脱硫弧菌属的相对丰度极显著升高(P<0.01)。
表5 单宁和裂壶藻粉对滩羊瘤胃菌群在属水平上相对丰度的影响

Table 5 Effects of tannin and Schizochytrium powder on rumen microflora relative abundance at genus level of Tan sheep%

项目
Items
对照组
Control group
试验Ⅰ组
Trial groupⅠ
试验Ⅱ组
Trial group Ⅱ
试验Ⅲ组
Trial groupⅢ
P
P-value
普雷沃氏菌属 Prevotella 17.93±9.21 30.18±20.11 27.66±12.04 25.35±11.40 0.485 0
理研菌科_RC9_肠道群
Rikenellaceae_RC9_gut_group
12.28±3.61Aab 16.80±13.30ABa 4.81±2.62Bab 2.49±2.29Bb 0.000 5
解琥珀酸菌属 Succiniclasticum 7.11±10.54 3.08±2.57 8.32±8.72 3.88±4.62 0.189 2
普雷沃氏菌科UCG-003
Prevotellaceae_UCG-003
3.31±4.15 2.82±0.85 7.23±4.09 3.98±3.26 0.307 2
琥珀酸弧菌属 Succinivibrio 1.14±1.77 1.24±1.53 2.72±5.11 1.19±1.70 0.496 9
未分类硒藻科
Unclassified_Selenomonadaceae
3.12±3.33 4.79±3.06 0.94±0.72 5.30±8.27 0.058 1
韦荣氏球菌科_UCG-001
Veillonellaceae_UCG-001
2.37±1.47ab 1.70±0.90a 5.09±3.86ab 3.79±1.53b 0.045 3
Norank_Muribaculaceae 2.42±1.06ab 1.24±0.73a 3.70±2.01b 4.68±3.51ab 0.016 9
奎因氏菌属 Quinella 4.76±5.69 5.90±9.67 0.45±0.77 0.45±0.55 0.118 4
Norank_F082 3.21±1.56 3.01±1.63 3.76±5.09 1.04±0.84 0.064 0
脱硫弧菌属 Desulfovibrio 1.65±0.73Bb 0.54±0.30Aa 2.91±2.49ABab 3.14±1.98Bb 0.005 5
普雷沃氏菌科UCG-001
Prevotellaceae_UCG-001
1.82±1.12 2.02±0.77 1.88±1.07 1.73±1.02 0.859 0
毛螺菌科_NK3A20_群
Lachnospiraceae_NK3A20_group
1.41±0.71 1.04±0.49 2.59±3.56 2.38±1.32 0.313 9
月形单胞菌属 Selenomonas 1.67±0.85 2.11±0.96 2.15±1.80 1.49±1.09 0.685 4
克里斯滕森菌科R-7群
Christensenellaceae_R-7_group
1.78±1.30 1.07±0.24 1.54±0.86 2.50±1.28 0.233 1
瘤胃球菌属 Ruminococcus 1.77±1.04 2.08±2.15 1.07±0.52 1.29±1.03 0.549 2
厌氧弧菌属 Anaerovibrio 1.36±0.94 0.76±0.39 1.70±1.36 1.79±0.72 0.069 2
UCG-002 1.37±0.77 0.79±0.35 1.05±0.96 2.05±3.42 0.645 9
Norank_Eubacterium_
coprostanoligenes_group
1.53±0.66 0.76±0.38 1.49±0.78 1.38±0.57 0.089 7
未排位硒藻科
Norank_Selenomonadaceae
1.43±1.03 0.72±0.66 1.20±0.90 1.27±0.36 0.288 6
Norank_UCG-010 1.21±0.57 0.76±0.46 1.14±1.23 0.62±0.70 0.274 7
依赖杆菌属 Fretibacterium 1.09±2.20 1.24±2.71 0.58±0.65 0.57±0.39 0.451 7
未分类毛螺菌科
Unclassified_Lachnospiraceae
1.24±0.94 0.45±0.23 0.80±0.36 0.84±0.27 0.062 8
UCG-004 0.73±0.92 0.83±0.64 0.90±1.52 0.62±0.44 0.761 0
未排位双歧杆菌科
Norank_Bifidobacteriaceae
0.94±1.44 0.22±0.26 0.14±0.26 1.68±3.41 0.338 2
NK4A214_group 1.29±0.91 0.45±0.20 0.43±0.29 0.64±0.53 0.203 1
丁酸弧菌属 Butyrivibrio 0.90±0.61 0.50±0.35 0.89±0.50 0.52±0.28 0.233 4
未分类普雷沃氏菌科
Unclassified_Prevotellaceae
0.50±0.57 0.57±0.42 1.22±0.68 0.49±0.36 0.119 3
未分类琥珀酸弧菌科
Unclassified_Succinivibrionaceae
0.08±0.06 1.08±1.47 0.53±0.41 1.04±1.56 0.170 1
未排位拟杆菌目_BS11_肠道群
Norank_Bacteroidales_BS11_gut_group
1.86±0.96Aa 0.58±0.97ABb 0.10±0.07Bab 0.04±0.05Bab 0.000 6
未排位拟杆菌目_RF16_群
Norank_Bacteroidales_RF16_group
0.77±0.32Aab 1.00±0.54ABa 0.47±0.19ABa 0.19±0.13Bb 0.002 6
图6 属水平上瘤胃菌群Circos图

Prevotella:普雷沃氏菌属;Others:其他;Rikenellaceae_RC9_gut_group:理研菌科_RC9_肠道群;Succiniclasticum:解琥珀酸菌属;Prevotellaceae_UCG-003:普雷沃氏菌科UCG-003;Succinivibrio:琥珀酸弧菌属;unclassified_Selenomonadaceae:未分类硒藻科:Veillonellaceae_UCG-001:韦荣氏球菌科_UCG-001;Quinella:奎因氏菌属;Desulfovibrio:脱硫弧菌属;Prevotellaceae_UCG-001:普雷沃氏菌科UCG-001;Lachnospiraceae_NK3A20_group:毛螺菌科_NK3A20_群;Selenomonas:月形单胞菌属;Christensenellaceae_R-7_group:克里斯滕森菌科R-7群;Ruminococcus:瘤胃球菌属;Anaerovibrio:厌氧弧菌属;norank_Selenomonadaceae:未排位硒藻科;Fretibacterium:依赖杆菌属;unclassified_Lachnospiraceae:未分类毛螺菌科;norank_Bifidobacteriaceae:未排位双歧杆菌科;Butyrivibrio:丁酸弧菌;unclassified_Prevotellaceae:未分类普雷沃氏菌科;unclassified_Succinivibrionaceae:未分类琥珀酸弧菌科:norank_Bacteroidales_BS11_gut_group:未排位拟杆菌目_BS11_肠道菌群;norank_Bacteroidales_RF16_group:未排位拟杆菌目_RF16_群。

Fig.6 Circos diagram of rumen microflora at genus level

2.3 瘤胃菌群功能预测分析(PICRUSt)

表6可知,在KEGG生物代谢一级通路水平上,各组滩羊的功能基因主要富集在新陈代谢(metabolism)、遗传信息处理(genetic information processing)和环境信息处理(environmental information processing)。每种功能基因在各组滩羊中相对丰度基本一致。在KEGG生物代谢二级通路水平上,各组滩羊瘤胃菌群功能丰度富集在前10条的二级通路依次为全局和概述图谱(global and overview maps)、碳水化合物代谢(carbohydrate metabolism)、氨基酸代谢(amino acid metabolism)、辅助因子和维生素的代谢(metabolism of cofactors and vitamins)、能量代谢(energy metabolism)、翻译(translation)、复制和修复(replication and repair)、信号转导(nucleotide metabolism)、膜运输(membrane transport)和聚糖的生物合成和代谢(glycan biosynthesis and metabolism)。其中,试验Ⅰ组的滩羊瘤胃菌群的氨基酸代谢功能通路相对丰度显著高于试验Ⅱ组(P<0.05)。
表6 滩羊瘤胃菌群功能丰度KEGG通路分析

Table 6 KEGG pathway analysis of rumen microflora functional abundance in Tan sheep

一级通路
Primary path
二级通路
Secondary pathway
KEGG二级通路功能丰度
KEGG secondary pathway functional abundance
对照组
Control
group
试验Ⅰ组
Trial
group Ⅰ
试验Ⅱ组
Trial
group Ⅱ
试验Ⅲ组
Trial group
P
P-value
全局和概述图谱
Global and overview maps
30 206 108.89
±1 676 409.68
31 436 318.54
±699 858.09
30 654 665.39
±628 738.85
31 019 102.18
±1 183 992.78
0.097 0
碳水化合物代谢
Carbohydrate metabolism
6 919 511.21
±354 391.18
7 375 558.05
±458 800.71
7 168 944.18
±134 058.53
716 8464.99
±489 127.54
0.073 0
新陈代谢
Metabolism
氨基酸代谢
Amino acid metabolism
5 406 665.69
±327 148.67ab
5 654 024.80
±162 557.93a
5 364 070.84
±112 269.65b
5 477 018.16
±162 090.01ab
0.025 0
辅助因子和维生素的代谢
Metabolism of cofactors and
vitamins
3 378 635.29
±287 067.78
3 486 585.29
±105 141.41
3 515 044.26
±135 315.20
3 506 620.93
±210 387.41
0.286 0
能量代谢
Energy metabolism
3 190 619.90
±188 163.85
3 325 915.58
±89 496.04
3 278 429.06
±82 889.59
3 197 341.15
±122 190.63
0.107 0
信号转导
Nucleotide metabolism
2 089 975.09
±142 454.36
2 221 464.72
±124 041.98
2 189 749.83
±81 015.36
2 167 253.72
±108 635.04
0.157 0
聚糖的生物合成和代谢
Glycan biosynthesis and
metabolism
1 393 552.81
±173 108.62
1 545 107.89
±170 211.65
1 560 158.27
±136 504.33
1 498 681.40
±188 853.94
0.084 0
遗传信息处理
Genetic
information
processing
翻译 Translation 2 753 874.95
±142 703.31
2 836 973.10
±33 430.51
2 801 879.46
±60 764.40
2 808 792.21
±84 413.81
0.086 0
复制和修复
Replication and repair
2 378 251.04
±125 355.66
2 469 981.21
±42 993.67
2 430 065.74
±52 986.17
2 423 873.01
±74 566.72
0.063 0
环境信息处理
Environmental
information
processing
膜运输
Membrane transport
1 758 953.53
±254 424.77
1 620 419.99
±257 991.50
1 705 501.99
±152 426.76
1 900 347.72
±228 610.61
0.130 0

3 讨论

生长性能是衡量动物生长速率最重要的指标,也是动物对饲粮中营养物质消化吸收情况的最终显现。刘绘汇等[16]研究发现,在羔羊的代乳粉中添加0.2%的单宁酸能够显著提高羔羊的采食量和平均日增重,与本试验研究结果一致。这是因为单宁对瘤胃蛋白有过瘤胃保护作用,其降低了蛋白质在瘤胃中的降解度,增加了肠道对蛋白质和氨基酸的吸收,提高氮素的利用率。同时由于过瘤胃蛋白含量增加,瘤胃菌群所需的营养物质减少,抑制了菌群的正常繁殖,改变了瘤胃菌群结构,降低了营养物质在瘤胃中的代谢效率,从而使得营养物质进入小肠被小肠消化吸收的含量增多,使得吸收更加充分,从长期来看,与滩羊总增重和平均日增重提高的结果相对应。此外,也有研究表明,单宁会增加空肠和回肠中的绒毛高度、促进肠道细胞的增殖、提高血清中总蛋白和球蛋白的含量、改善肠道完整性、增强机体蛋白质代谢和免疫力、改善了生长性能[17]。在本试验中,试验Ⅰ组瘤胃内脱硫菌门相对丰度的下降再次验证了这一结果。徐晨晨等[18]在柴达木福牛的饲粮中添加100 g/d DHA微藻粉,结果显示该牛的平均日增重增加,这与本试验的结果一致。这可能与DHA会激活蛋白激酶/哺乳动物雷帕霉素靶蛋白(Akt/mTOR)信号通路,增强肌肉蛋白质合成[19],降低瘤胃中氨基酸代谢有关。在本试验中,试验Ⅰ组瘤胃内碳水化合物代谢通路、能量代谢通路和聚糖的生物合成和代谢水平要高于试验Ⅲ组,继而导致了试验Ⅰ组对生长性能提升的效果要优于试验Ⅲ组。
瘤胃是反刍动物主要的消化器官,就像是一个密闭的厌氧发酵罐,其内栖息着庞大的微生物群落,包括细菌、真菌、原虫等。微生物菌群能将不能被反刍动物直接消化吸收的纤维素和非蛋白氮等,转变为可吸收的短链脂肪酸和含氮物质等代谢产物,为反刍动物的生长发育提供必须的物质和能量。大量研究证实,反刍动物瘤胃中的优势菌群为拟杆菌门和厚壁菌门,其在瘤胃发酵过程中起着重要的作用[20-21]。拟杆菌门为反刍动物瘤胃中的第1优势菌群,主要承担着分解蛋白质和碳水化合物、维持胃肠道正常生理功能的作用[22]。厚壁菌门作为第2优势菌群,主要承担降解纤维素和半纤维素、参与能量代谢等[23]。有研究发现,厚壁菌门相对丰度增加,会使得拟杆菌门相对丰度降低,从而造成代谢紊乱[24]。常玮学等[25]发现,在秦川牛的饲粮中添加水解单宁会增加拟杆菌门的相对丰度,降低厚壁菌门的相对丰度。Zhao等[26]研究显示,在绵羊饲粮中添加蒙古葱精油也会增加拟杆菌门的相对丰度,降低厚壁菌门的相对丰度,这与本试验的结果一致。在本试验中,添加0.4%单宁+2.0%裂壶藻粉组出现了第3优势菌群——变形菌门,变形菌门中除含有纤维素降解菌、半纤维素降解菌和蛋白质降解菌等外,还包括许多致病菌[27]。所以同时添加单宁和裂壶藻粉及其添加量对滩羊瘤胃菌群的影响还需要进一步的试验分析。
脱硫菌门是一种肠道有害菌,可以分解短链脂肪酸[28],使机体炎性因子水平升高,并能穿过肠道黏液层在肠道中定植,肠道中脱硫菌门丰度较高时,会产生硫化氢[29]损伤肠道上皮细胞,破坏肠道屏障功能[30],引发溃疡性结肠炎[31]。疣微菌门可以分解多糖类物质,并产生短链脂肪酸,具有抗炎特性,能够有效增强哺乳动物瘤胃及肠道的免疫功能[32]。在本试验中,与对照组相比,试验Ⅰ组脱硫菌门的相对丰度极显著降低,这表明单宁可能通过降低脱硫菌门的相对丰度,改善滩羊的胃肠道健康。虽然试验Ⅲ组可能对滩羊瘤胃健康状况存在不利影响,但同时疣微菌门的相对丰度也显著提高了,由此可能起到了一个中和的作用,使滩羊瘤胃健康状况保持在一个较好的状态。同时,在本试验中还出现了Patescibacteria、浮霉菌门和WPS-2,目前它们在滩羊瘤胃中的作用鲜有报道,探究这些细菌是不是滩羊瘤胃中特有的菌群,或许可作为下一步的研究方向。
在本试验中,普雷沃氏菌属和理研菌科_RC9_肠道群为优势菌属。它们都属于拟杆菌门,可促进胃肠道中碳水化合物的消化吸收,在琥珀酸和丙酸产生的过程中起着重要的作用[33]。与对照组相比,试验Ⅰ组的普雷沃氏菌属和理研菌科_RC9_肠道群相对丰度增加,碳水化合物和能量代谢通路相对丰度增加,表明添加单宁可能会为滩羊提供更多的能量,进而促进其增重。与对照组相比,试验Ⅱ、Ⅲ组的普雷沃氏菌属相对丰度增加,理研菌科_RC9_肠道群相对丰度显著下降,这与高栋[34]的研究结果一致。卓萍等[35]研究发现,韦荣氏球菌可将乳酸转化为乙酸和丙酸,起到改善胃肠道内环境的作用。张莉[36]研究表明,韦荣氏球菌科与氨基酸、辅酶、能量和维生素的代谢,糖苷键代谢及其次级代谢产物呈正相关。在本试验中,与试验Ⅰ组相比,试验Ⅲ组的韦荣氏球菌科_UCG-001相对丰度显著增加,表明添加裂壶藻粉可以改善因单宁对滩羊代谢造成的不利影响。Yang等[37]研究发现,norank_Muribaculaceae是降胆固醇菌属,其与粪便中结合胆汁酸的水平呈负相关。在本试验中,与试验Ⅰ组相比,试验Ⅱ组的norank_Muribaculaceae相对丰度上升,这可能与裂壶藻粉中的多糖类物质有关。此外,基于当前细菌数据库,本研究在滩羊瘤胃菌群内还检测到大量未被分类和排位鉴定的菌属,表明滩羊瘤胃中可能存在一些特定的菌群,同时也反映了目前对微生物区系研究还不足够的事实,在今后的研究中有待于进一步挖掘。

4 结论

饲粮中添加单宁和裂壶藻粉会提高滩羊的平均日增重,调节瘤胃菌群结构,提高碳水化物化合物和能量代谢等。本试验中,在饲粮中单独添加0.4%单宁的效果最佳,同时添加0.4%单宁和2.0%裂壶藻粉效果次之,而单独添加2.0%裂壶藻粉的效果不太明显。
[1]
NOOROLAHI Z, SAHARI M A, BARZEGAR M, et al. Tannin fraction of pistachio green hull extract with pancreatic lipase inhibitory and antioxidant activity[J]. Journal of Food Biochemistry, 2020, 44(6):e13208.

[2]
GONTIJO D C, GONTIJO P C, BRANDÃO G C, et al. Antioxidant study indicative of antibacterial and antimutagenic activities of an ellagitannin-rich aqueous extract from the leaves of Miconia latecrenata[J]. Journal of Ethnopharmacology, 2019, 236:114-123.

DOI

[3]
SONG D, ZHAO J B, DENG W X, et al. Tannic acid inhibits NLRP3 inflammasome-mediated IL-1β production via blocking NF-κB signaling in macrophages[J]. Biochemical and Biophysical Research Communications, 2018, 503(4):3078-3085.

DOI PMID

[4]
PONG L Y, YEW P N, LEE W L, et al. Anti-dengue virus serotype 2 activity of tannins from porcupine dates[J]. Chinese Medicine, 2020, 15(1):49.

DOI

[5]
ISHLAK A, GÜNAL M, ABUGHAZALEH A A. The effects of cinnamaldehyde,monensin and quebracho condensed tannin on rumen fermentation,biohydrogenation and bacteria in continuous culture system[J]. Animal Feed Science and Technology, 2015, 207:31-40.

DOI

[6]
YU F, BARRY T N, MCNABB W C, et al. Effect of bound condensed tannin from cottonseed upon in situ protein solubility and dry matter digestion in the rumen[J]. Journal of the Science of Food and Agriculture, 1995, 69(3):311-319.

DOI

[7]
MAPIYE C, ALDAI N, TURNER T D, et al. The labile lipid fraction of meat:from perceived disease and waste to health and opportunity[J]. Meat Science, 2012, 92(3):210-220.

DOI

[8]
DOS SANTOS S K, DE FÁTIMA FRANÇA BIZ J, SALGADO J A, et al. Intake and performance of growing lambs supplemented with quebracho tannins[J]. Tropical Animal Health and Production, 2022, 54(1):71.

DOI PMID

[9]
朱辉权. 饲喂DHA微藻粉对山羊乳品质的影响[D]. 硕士学位论文. 北京: 中国农业科学院, 2021:16-33.

ZHU H Q. Effect of feeding DHA microalgae powder on goat milk quality[D]. Master’s Thesis. Beijing: Chinese Academy of Agricultural Sciences, 2021:16-33. (in Chinese)

[10]
徐晨晨. 富含DHA的微藻对牦牛肉品质及脂质变化影响机制的研究[D]. 博士学位论文. 北京: 中国农业科学院, 2021.

XU C C. The effect mechanism of DHA-rich microalgae on the quality and lipid changes of yak meat[D]. Ph.D.Thesis. Beijing: Chinese Academy of Agricultural Sciences, 2021. (in Chinese)

[11]
MAVROMMATIS A, THEODOROU G, POLITIS I, et al. Schizochytrium sp. dietary supplementation modify Toll-like receptor 4 (TLR4) transcriptional regulation in monocytes and neutrophils of dairy goats[J]. Cytokine, 2021, 148:155588.

DOI

[12]
齐明江. 栗木单宁对育肥滩羊瘤胃发酵、生产性能及肉品质的影响[D]. 硕士学位论文. 银川: 宁夏大学, 2022:32-33.

QI M J. Effects of chestnut tannin on rumen fermentation,production performance and meat quality of fattening Tan sheep[D]. Master’s Thesis. Yinchuan: Ningxia University, 2022:32-33. (in Chinese)

[13]
李海庆. 日粮不饱和脂肪酸对滩羊体脂CLA调控作用及机理研究[D]. 博士学位论文. 银川: 宁夏大学, 2019:72-74.

LI H Q. Study on effects and mechanisms of dietary unsaturated fatty acids on tissue conjugated linoleic acid (CLA) synthesis of Tan sheep[D]. Ph.D.Thesis. Yinchuan: Ningxia University, 2019:72-74. (in Chinese)

[14]
KAMEL H E, AI-DOBAIB S N, SALEM A Z. Dietary supplementation of sunflower oil and quebracho tannins in sheep feeding:in vivo nutrient digestibility,nitrogen utilization and in vitro ruminal degradation kinetics[J]. Journal of the Science of Food and Agriculture, 2019, 99(9):4211-4217.

DOI

[15]
LIU H, PUCHALA R, LESHURE S, et al. Effects of lespedeza condensed tannins alone or with monensin,soybean oil,and coconut oil on feed intake,growth,digestion,ruminal methane emission,and heat energy by yearling Alpine doelings[J]. Journal of Animal Science, 2019, 97(2):885-899.

DOI

[16]
刘绘汇, 孙康, 范慧玉, 等. 代乳粉中添加单宁酸对湖羊羔羊生长性能、养分表观消化率和肌肉脂肪酸组成的影响[J]. 动物营养学报, 2021, 33(8):4520-4532.

DOI

LIU H H, SUN K, FAN H Y, et al. Effects of tannic acid addition in milk replacer on growth performance,nutrient apparent digestibility and muscle fatty acid composition of Hu lambs[J]. Chinese Journal of Animal Nutrition, 2021, 33(8):4520-4532. (in Chinese)

[17]
ZHAO M D, DI L F, TANG Z Y, et al. Effect of tannins and cellulase on growth performance,nutrients digestibility,blood profiles,intestinal morphology and carcass characteristics in Hu sheep[J]. Asian-Australasian Journal of Animal Sciences, 2019, 32(10):1540-1547.

DOI

[18]
徐晨晨, 李慧, 张寿, 等. 富含DHA微藻对柴达木福牛生长性能和血清抗氧化指标的影响[J]. 中国畜牧兽医, 2021, 48(6):2074-2081.

XU C C, LI H, ZHANG S, et al. Effect of dietary DHA-rich microalgae on growth performance and serum antioxidant indices of qaidamford cattle[J]. China Animal Husbandry & Veterinary Medicine, 2021, 48(6):2074-2081. (in Chinese)

[19]
窦露, 刘畅, 杨致昊, 等. 动物肌肉组织蛋白质代谢调控的研究进展[J]. 动物营养学报, 2022, 34(1):39-50.

DOI

DOU L, LIU C, YANG Z H, et al. Research progress on regulation of protein metabolism in animal muscle tissue[J]. Chinese Journal of Animal Nutrition, 2022, 34(1):39-50. (in Chinese)

[20]
马小勇, 谭义洲, 任稳稳, 等. 犏牛、黄牛和娟姗牛瘤胃菌群结构比较及功能预测研究[J]. 西北农林科技大学学报(自然科学版), 2023, 51(8):1-10.

MA X Y, TAN Y Z, REN W W, et al. Comparison of rumen microbiota structure and functional prediction among cattle yak,cattle and Jersey[J]. Journal of Northwest A & F University (Natural Science), 2023, 51(8):1-10. (in Chinese)

[21]
马友记, 陈鹏飞, 马青, 等. 不同运动量对滩羊瘤胃菌群多样性的影响[J/OL]. 畜牧兽医学, 2023:1-14.[2023-07-14]. http://kns.cnki.net/kcms/detail/11.1985.S.20230303.1014.002.h ml.

MA Y J, CHEN P F, MA Q, et al. Effects of different exercise amounts on rumen microflora diversity of Tan sheep[J]. Acta Veterinaria et Zootechnica Sinica, 2023:1-14.[2023-07-14]. http://kns.cnki.net/kcms/detail/11.1985.S.20230303.1014.002.html. in Chinese)

[22]
HESS M, SCZYRBA A, EGAN R, et al. Metagenomic discovery of biomass-degrading genes and genomes from cow rumen[J]. Science, 2011, 331(6016):463-467.

DOI PMID

[23]
HOOK S E, STEELE M A, NORTHWOOD K S, et al. Impact of subacute ruminal acidosis (SARA) adaptation and recovery on the density and diversity of bacteria in the rumen of dairy cows[J]. FEMS Microbiology Ecology, 2011, 78(2):275-284.

DOI PMID

[24]
GROVER M. Role of gut pathogens in development of irritable bowel syndrome[J]. Indian Journal of Medical Research, 2014, 139(1):11-18.

PMID

[25]
常玮学, 杨英超, 夏志军, 等. 不同添加量的植物水解单宁对秦川肉牛血清生化指标和瘤胃消化指标、瘤胃微生物区系的影响[J]. 动物营养学报, 2022, 34(3):1642-1654.

DOI

CHANG W X, YANG Y C, XIA Z J, et al. Effects of different addition amounts of plant hydrolyzed tannins on serum biochemical indexes,rumen digestion indexes and rumen microflora of Qinchuan beef cattle[J]. Chinese Journal of Animal Nutrition, 2022, 34(3):1642-1654. (in Chinese)

[26]
ZHAO Y X, ERDENE K, BAO Z B, et al. Effects of Allium mongolicum regel essential oil supplementation on growth performance,nutrient digestibility,rumen fermentation,and bacterial communities in sheep[J]. Frontiers in Veterinary Science, 2022, 9:926721.

DOI

[27]
BYNDLOSS M X, BÄUMLER A J. The germ-organ theory of non-communicable diseases[J]. Nature Reviews Microbiology, 2018, 16(2):103-110.

DOI PMID

[28]
GIBSON G R, MACFARLANE G T, CUMMINGS J H. Occurrence of sulphate-reducing bacteria in human faeces and the relationship of dissimilatory sulphate reduction to methanogenesis in the large gut[J]. Journal of Applied Bacteriology, 1988, 65(2):103-111.

DOI PMID

[29]
SCANLAN P D, SHANAHAN F, MARCHESI J R. Culture-independent analysis of desulfovibrios in the human distal colon of healthy,colorectal cancer and polypectomized individuals[J]. FEMS Microbiology Ecology, 2009, 69(2):213-221.

DOI

[30]
ROWAN F E, DOCHERTY N G, COFFEY J C, et al. Sulphate-reducing bacteria and hydrogen sulphide in the aetiology of ulcerative colitis[J]. British Journal of Surgery, 2009, 96(2):151-158.

DOI

[31]
胡雪黎, 田力, 李鸿, 等. 土家药三颗针对溃疡性结肠炎小鼠肠道菌群的影响[J]. 天然产物研究与开发, 2022, 34(12):2069-2076.

HU X L, TIAN L, LI H, et al. Effect of Tujia medicine berberidis radix on intestinal flora in mice with ulcerative colitis[J]. Natural Product Research and Development, 2022, 34(12):2069-2076. (in Chinese)

[32]
DERRIEN M, VAN BAARLEN P, HOOIVELD G, et al. Modulation of mucosal immune response,tolerance,and proliferation in mice colonized by the mucin-degrader Akkermansia muciniphila[J]. Frontiers in Microbiology, 2011, 2:166.

[33]
王庆, 张巧娥, 张转弟, 等. 复合菌颗粒料对犊牛瘤胃发酵参数及菌群结构的影响[J]. 中国饲料, 2022(19):55-61.

WANG Q, ZHANG Q E, ZHANG Z D, et al. Effects of compound bacterial granules on rumen fermentation parameters and microflora structure of calves[J]. China Feed, 2022(19):55-61. (in Chinese)

[34]
高栋. 添加不同形式亚麻油对肉羊肉品质、肌肉脂肪酸、血清生化指标、瘤胃发酵指标和瘤胃微生物的影响[D]. 硕士学位论文. 呼和浩特: 内蒙古农业大学, 2020:27-31.

GAO D. Effects of different forms of linseed oil on meat and mutton quality,muscle fatty acid,serum biochemical index,rumen fermentation index and rumen microbial diversity[D]. Master’s Thesis. Hohhot: Inner Mongolia Agricultural University, 2020:27-31. (in Chinese)

[35]
卓萍, 刘威, 刘君琴, 等. 一株人消化道中韦荣氏球菌的分离、鉴定及其代谢特性研究[J]. 微生物学通报, 2016, 43(6):1253-1261.

ZHUO P, LIU W, LIU J Q, et al. Isolation,identification and metabolism of a Veillonella strain in human gut[J]. Microbiology, 2016, 43(6):1253-1261. (in Chinese)

[36]
张莉. 日粮纤维对仔猪肠道屏障功能的影响及调控机制的研究[D]. 博士学位论文. 北京: 中国农业科学院, 2018:44-58.

ZHANG L. Effects and the regulatory mechanism of dietary fiber on intestinal barrier function in piglets[D]. Ph.D.Thesis. Beijing: Chinese Academy of Agricultural Sciences, 2018:44-58. (in Chinese)

[37]
YANG C W, HUANG S Y, LIN Z G, et al. Polysaccharides from Enteromorpha prolifera alleviate hypercholesterolemia via modulating the gut microbiota and bile acid metabolism[J]. Food & Function, 2022, 13(23):12194-12207.

文章导航

/