研究论文

发酵枳实残渣对仔猪生长性能、抗氧化能力和肠道健康的影响

  • 殷运菊 , 1, 2 ,
  • 史寒婧 1, 3 ,
  • 陈思思 1, 4 ,
  • 吴宜洋 2 ,
  • 周媛媛 2 ,
  • 汤赫 5 ,
  • 汤佳 5 ,
  • 郭秋平 1 ,
  • 李凤娜 , 1, 4, *
展开
  • 1 中国科学院亚热带农业生态研究所,亚热带农业生态过程重点实验室,长沙 410125
  • 2 湖南农业大学动物科学技术学院,长沙 410128
  • 3 湖南师范大学生命科学学院,动物肠道功能调控湖南省重点实验室,长沙 410081
  • 4 中国科学院大学现代农业科学学院,北京 100049
  • 5 张家界继源科技有限公司,张家界 427099
* 李凤娜,研究员,博士生导师,E-mail:

殷运菊(1994—),女,贵州六盘水人,硕士研究生,从事动物营养学与饲料资源开发与利用研究。E-mail:

Copy editor: 武海龙

收稿日期: 2023-07-13

  网络出版日期: 2024-01-12

基金资助

湖南省重点研发计划项目(2022NK2026)

湖南省科技创新领军人才计划资助(2021RC4039)

Effects of Fermented Fructus Aurantii Immaturus Residue on Growth Performance, Antioxidant Capacity and Intestinal Health of Piglets

  • YIN Yunju , 1, 2 ,
  • SHI Hanjing 1, 3 ,
  • CHEN Sisi 1, 4 ,
  • WU Yiyang 2 ,
  • ZHOU Yuanyuan 2 ,
  • TANG He 5 ,
  • TANG Jia 5 ,
  • GUO Qiuping 1 ,
  • LI Fengna , 1, 4, *
Expand
  • 1 Key Laboratory of Agro-Ecological Processes in Subtropical Region, Institute of Subtropical Agriculture, Chinese Academy of Sciences, Changsha 410125, China
  • 2 College of Animal Science and Technology, Hunan Agricultural University, Changsha 410128, China
  • 3 Hunan Provincial Key Laboratory of Animal Intestinal Function Regulation, College of Life Sciences, Hunan Normal University, Changsha 410081, China
  • 4 College of Modern Agricultural Sciences, University of Chinese Academy of Sciences, Beijing 100049, China
  • 5 Zhangjiajie Jiyuan Technology Co., Ltd., Zhangjiajie 427099, China
* professor, E-mail:

Received date: 2023-07-13

  Online published: 2024-01-12

摘要

本试验旨在探究发酵枳实残渣对仔猪生长性能、抗氧化能力和肠道健康的影响。选取32头体重为(7.65±0.18) kg杜×长×大三元杂交仔猪,随机分为4组,每组8个重复,每个重复1头猪。各组分别饲喂发酵枳实残渣添加水平为0(对照组)、4%(4%FF组)、8%(8%FF组)、12%(12%FF组)的试验饲粮。试验期30 d。结果表明:1)与对照组相比,8%FF组的平均日增重和平均日采食量显著提高(P<0.05)。2)与对照组相比,8%FF组的血清总蛋白(TP)、免疫球蛋白A(IgA)、免疫球蛋白G(IgG)、免疫球蛋白M(IgM)含量和超氧化物歧化酶(SOD)、过氧化氢酶(CAT)、谷胱甘肽过氧化物酶(GSH-Px)活性显著提高(P<0.05),4%FF、8%FF、12%FF组的血清总抗氧化能力(T-AOC)显著提高(P<0.05),4%FF和8%FF组的血清丙二醛(MDA)含量显著降低(P<0.05)。3)与对照组相比,8%FF组的空肠绒毛高度、杯状细胞数量和绒毛高度/隐窝深度显著提高(P<0.05),空肠隐窝深度显著降低(P<0.05)。4)与对照组相比,8%FF和12%FF组的空肠闭锁小带蛋白-1(ZO-1)、超氧化物歧化酶1(SOD1)和核因子E2相关因子2(Nrf2)的mRNA相对表达水平显著提高(P<0.05),8%FF组的空肠封闭蛋白(Occludin)的mRNA相对表达水平显著提高(P<0.05)。5)与对照组相比,8%FF和12%FF组的结肠拟杆菌门(Bacteroidetes)相对丰度显著提高(P<0.05),结肠厚壁菌门(Firmicutes)相对丰度显著降低(P<0.05);4%FF和8%FF组的结肠乳杆菌属(Lactobacillus)相对丰度显著提高(P<0.05),12%FF组的结肠普氏菌属(Prevotella)相对丰度显著提高(P<0.05),4%FF、8%FF和12%FF组的结肠链球菌属(Streptococcus)相对丰度显著降低(P<0.05)。综上所述,饲粮中添加发酵枳实残渣对仔猪生长性能无负面影响,并且能提高机体抗氧化能力,改善肠道形态,增加肠道微生物多样性,最终改善仔猪的生长性能。本试验条件下,仔猪饲粮中发酵枳实残渣添加水平以8%为宜。

本文引用格式

殷运菊 , 史寒婧 , 陈思思 , 吴宜洋 , 周媛媛 , 汤赫 , 汤佳 , 郭秋平 , 李凤娜 . 发酵枳实残渣对仔猪生长性能、抗氧化能力和肠道健康的影响[J]. 动物营养学报, 2024 , 36(1) : 186 -198 . DOI: 10.12418/CJAN2024.018

Abstract

This experiment was conducted to investigate the effects of fermented fructus aurantii immaturus residue on growth performance, antioxidant capacity and intestinal health of piglets. Thirty-two Duroc×Landrace×Large White hybrid piglets with the body weight of (7.65±0.18) kg were randomly divided into 4 groups with 8 replicates per group and 1 piglet per replicate. Piglets in 4 group were fed experimental diets which the fermented fructus aurantii immaturus residue supplemental levels were 0 (control group), 4% (4%FF group), 8% (8%FF group) and 12% (12%FF group), respectively. The experiment lasted for 30 days. The results showed as follows: 1) compared with the control group, the average daily gain and average daily feed intake of 8%FF group were significantly increased (P<0.05). 2) Compared with the control group, the serum total protein (TP), immunoglobulin A (IgA), immunoglobulin G (IgG), immunoglobulin M (IgM) contents and superoxide dismutase (SOD), catalase (CAT), glutathione peroxidase (GSH-Px) activities of 8%FF group were significantly increased (P<0.05), the serum total antioxidant capacity (T-AOC) of 4%FF, 8%FF and 12%FF groups was significantly increased (P<0.05), and the serum malondialdehyde (MDA) content of 4%FF and 8%FF groups was significantly decreased (P<0.05). 3) Compared with the control group, the jejunal villus height, goblet cell number and villus height/crypt depth of 8%FF group were significantly increased (P<0.05), and the jejunal crypt depth was significantly decreased (P<0.05). 4) Compared with the control group, the mRNA relative expression levels of zonula occluden-1 (ZO-1), superoxide dismutase 1 (SOD1) and nuclear factor E2 related factor 2 (Nrf2) in jejunum of 8%FF and 12%FF groups were significantly increased (P<0.05), and the jejunal Occludin mRNA relative expression level of 8%FF group was significantly increased (P<0.05). 5) Compared with the control group, the colonic Bacteroidetes relative abundance of 8%FF and 12%FF groups was significantly increased (P<0.05), and the colonic Firmicutes relative abundance was significantly decreased (P<0.05); the colonic Lactobacillus relative abundance of 4%FF and 8%FF groups was significantly increased (P<0.05), the colonic Prevotella relative abundance of 12%FF group was significantly increased (P<0.05), and the colonic Streptococcus relative abundance of 4%FF, 8%FF and 12%FF groups was significantly decreased (P<0.05). In conclusion, dietary fermented fructus aurantii immaturus residue has no negative effect on the growth performance of piglets, and can improve the body antioxidant capacity and intestinal morphology, increase the intestinal microbial diversity, and ultimately improve the growth performance of piglets. Under the conditions of this experiment, the dietary suitable fermented fructus aurantii immaturus residue level is 8%.

枳实(fructus aurantii immaturus,FAI)是一种酸橙或甜橙的干燥幼果。《中国药典》1990年收载枳实基原为芸香科植物酸橙及其栽培变种(黄皮酸橙、代代花、朱栾、塘橙等),主产于湖南、江西、四川、湖北、浙江等地,以湖南产量最大,占全国产量的40%~60%。枳实的生物活性成分主要包括黄酮类、挥发油类和生物碱类化合物,其中最能体现枳实特征的活性成分是黄酮类化合物[1]。枳实味苦性凉,归脾、胃经,可健脾破气,并能消除积食、祛痰除痞;临床上经常与其他药物配伍使用,治疗胃下垂、积食消化停滞、便秘腹痛不良症状[2]。胡源祥等[3]研究表明,枳实中的柚皮苷、新橙皮苷、辛弗林可升高脾虚型大鼠血清胃泌素和血浆胃动素水平,从而达到促进胃肠运动的效果。枳实中川陈皮素通过维持豚鼠回肠黏膜屏障完整性、促进胃运动防止内源性乙酰胆碱和组胺的作用,进而达到抗溃疡的作用[4]。舒一崧[5]证实枳实可逆转乙酰氨基酚诱导的肝脏损伤中脂质代谢紊乱,调节脂质代谢结合介导的多靶向信号通路,发挥保肝作用。此外,枳实提取物可以提高糖尿病小鼠肝脏抗氧化酶活性,抑制脂质过氧化物反应[6]。现代研究表明,枳实的药理作用表现为调节胃肠道、抗炎、保肝、抗溃疡等,但其在养猪生产中的应用鲜有研究。湖南省枳实资源丰富,枳实经提取后,其残渣中的有效活性成分约含30%,可作为畜禽非常规饲料资源开发和利用[7]。因此,本试验为了保证枳实残渣有效成分的高效利用,进一步提高残渣的营养价值,在将其饲喂之前进行微生物发酵处理,探究不同发酵枳实残渣添加水平对仔猪生长性能、抗氧化能力和肠道健康的影响,以期为枳实在畜牧生产中的应用提供理论依据和技术支撑。

1 材料与方法

1.1 试验材料

将枳实残渣(湿)与豆粕、统糠(谷壳)、麦麸、玉米粉、复合发酵液(以乳酸菌为主)按照一定比例混合后发酵7 d,发酵枳实残渣配方如表1所示,枳实残渣发酵前后常规养分含量如表2所示。
表1 发酵枳实残渣配方

Table 1 Formula of fermented fructus aurantii immaturus residue%

原料Ingredients 含量Content
枳实残渣(湿)
Fructus aurantii immaturus residue (wet)
40.00
豆粕Soybean meal 25.00
统糠(谷壳) Rice bran (chaff) 20.00
麦麸Wheat bran 8.00
玉米粉Corn meal 5.00
复合发酵液Compound fermentation broth 2.00
合计Total 100.00
表2 枳实残渣发酵前后常规养分含量(鲜物质基础)

Table 2 Conventional nutrient contents of fructus aurantii immaturus residue before and after fermentation (fresh matter basis)%

项目
Items
发酵前
Before
fermentation
发酵后
After
fermentation
水分Moisture 60.29 61.00
干物质Dry matter 39.71 39.01
粗蛋白质Crude protein 6.52 6.26
粗脂肪Crude fat 1.37 1.52
粗纤维Crude fiber 9.14 9.25
粗灰分Crude ash 3.79 3.80
钙Calcium 0.31 0.31
总磷Total phosphorus 0.19 0.19

1.2 试验设计

选用32头体况良好、体重[(7.65±0.18) kg]接近的杜×长×大三元杂交仔猪,采用单因素试验设计,按试验猪体重及遗传背景基本一致的原则,随机分成4组,每组8个重复,每个重复1头猪。各组分别饲喂发酵枳实残渣添加水平为0(对照组,CON组)、4%(4%FF组)、8%(8%FF组)、12%(12%FF组)的试验饲粮。试验期30 d。

1.3 试验饲粮及饲养管理

试验采用玉米-豆粕型饲粮,参考NRC(2012)设计,发酵枳实残渣主要替代玉米,各组试验饲粮等氮等能。试验饲粮组成及营养水平如表3所示。试验猪单栏饲养,全程采用粉料饲喂,自由采食和饮水。
表3 试验饲粮组成及营养水平(干物质基础)

Table 3 Composition and nutrient levels of experimental diets (DM basis) %

项目
Items
发酵枳实残渣添加水平
Fermented fructus aurantii immaturus residue
supplemental levels/%
0 4 8 12
原料Ingredients
玉米Corn 66.29 62.90 59.33 55.57
豆粕Soybean meal 19.75 18.65 17.90 17.30
乳清粉Whey mist 4.30 4.30 4.30 4.30
鱼粉Fish meal 4.00 4.00 4.00 4.00
大豆油Soybean oil 2.30 2.60 2.90 3.25
发酵枳实残渣Fermented fructus aurantii immaturus residue 4.00 8.00 12.00
赖氨酸盐酸盐Lysine·HCl 0.50 0.62 0.64 0.65
蛋氨酸Methionine 0.12 0.19 0.19 0.19
碳酸钙CaCO3 0.74 0.74 0.74 0.74
石粉Limestone 0.70 0.70 0.70 0.70
食盐NaCl 0.30 0.30 0.30 0.30
预混料Premix1) 1.00 1.00 1.00 1.00
合计Total 100.00 100.00 100.00 100.00
营养水平Nutrient levels2)
消化能Digestion energy/(MJ/kg) 14.63 14.46 14.33 14.21
粗蛋白质Crude protein 16.85 17.10 17.09 16.87
粗脂肪Crude fat 0.90 0.93 1.07 0.96
粗纤维Crude fiber 6.56 6.47 6.48 6.46
赖氨酸Lysine 1.24 1.23 1.23 1.24
蛋氨酸+半胱氨酸Methionine+cystine 0.68 0.67 0.67 0.69
钙Calcium 0.57 0.57 0.55 0.60
总磷Total phosphorus 0.54 0.54 0.55 0.57

1)预混料为每千克饲粮提供 Premix provided the following per kg of diets: VA 6 000 IU,VD3 4 000 IU,VE 40 IU,VK3 4 mg,VB1 6 mg,VB2 12 mg,VB6 6 mg,VB12 0.05 mg,生物素 biotin 0.2 mg,叶酸 folic acid 2 mg,烟酸 niacin 50 mg,D-泛酸钙 D-calcium pantothenate 25 mg,Cu 150 mg,Fe 100 mg,Mn 40 mg,Zn 100 mg,I 0.5 mg,Se 0.3 mg。

2)消化能为计算值,发酵枳实残渣的消化能参考柑橘渣的消化能计算[8];其他为实测值。Digestible energy was a calculated value, and the digestible energy of fermented fructus aurantii immaturus residue was calculated with reference to the digestible energy of citrus residue[8]; while the others were measured values.

1.4 屠宰与样品采集

试验结束时,所有猪禁食12 h后进行屠宰取样。屠宰前,颈静脉采集血样放入5 mL采血管中,室温静置30 min后于3 000×g、4 ℃条件下离心10 min,取上清置于1.5 mL离心管中,液氮速冻后转移至-80 ℃冰箱保存待测。取空肠(中段)组织、结肠(后段)内容物,多聚甲醛固定样品1份,液氮速冻样品2份,样品液氮速冻后转移至-80 ℃冰箱保存待测。

1.5 指标测定与方法

1.5.1 饲粮营养水平

用自动纤维分析仪(FT12,Gerhardt公司,德国)测定粗纤维含量;用微波消解法测定钙和总磷含量,所用仪器为电感耦合等离子体光谱仪(5110 ICP-OES,Agilent公司,美国);用凯氏定氮法测定粗蛋白质含量,所用仪器为流动注射仪(AA3,Seal公司,德国);按照GB/T 5009.6—2016的方法,用索氏抽提法测定粗脂肪含量,所用仪器为全自动索氏抽提仪(SOX416,Soxtherm公司,德国);根据饲料中常规养分含量计算消化能[9]

1.5.2 生长性能

分别在试验开始和结束时称重,每天记录猪的采食量和饲料损耗量,计算得出平均日增重(average daily gain,ADG)、平均日采食量(average daily feed intake,ADFI)和料重比(feed/gain,F/G)。

1.5.3 血清生化、抗氧化和免疫指标

测定前,取血清样品解冻,摇匀后取500 μL血清样品,用全自动生化分析仪(CobasC311,Roche公司,瑞士)和试剂盒(北京利德曼生物技术有限公司)测定血清总蛋白(total protein,TP)、白蛋白(albumin,ALB)、尿素氮(urea nitrogen,UN)、葡萄糖(glucose,GLU)、肌酐(creatinine,CRE)和总胆红素(total bilirubin,TBIL)含量。严格按照酶联免疫吸附试验(ELISA)试剂盒(长沙奥基生物科技有限公司)说明书检测血清谷胱甘肽过氧化物酶(glutathione peroxidase,GSH-Px)、超氧化物歧化酶(superoxide dismutase,SOD)、过氧化氢酶(catalase,CAT)活性和丙二醛(malonaldehyde,MDA)、免疫球蛋白A(immunoglobulin A,IgA)、免疫球蛋白G(immunoglobulin G,IgG)、免疫球蛋白M(immunoglobulin M,IgM)含量及总抗氧化能力(total antioxidant capacity,T-AOC)。

1.5.4 空肠组织形态

空肠组织形态检测参考Nosworthy等[10]的苏木精-伊红(HE)染色法,将固定好的空肠样品制成组织切片,显微镜下观察形态结构并拍照,测量每个组织切片上8~10根形态完整的绒毛高度(villus height,VH)、隐窝深度(crypt depth,CD)和杯状细胞数量,并计算绒毛高度/隐窝深度(V/C)。

1.5.5 空肠抗氧化和肠道形态相关基因mRNA表达

取空肠样品,加液氮在研钵中充分研磨,迅速转入加有1 mL Trizol的1.5 mL无菌无酶EP管中,在超净工作台内进行总RNA的提取,提取完成测RNA的浓度和纯度,吸光度(OD)260/OD280在1.8~2.2为合格样品,将所有样品RNA浓度调整到1 000 ng/μL,再用Evo M-MLV反转录试剂盒(湖南艾科瑞生物工程有限公司)反转录成cDNA。使用SYBR Green Premix ProTaq HS qPCR试剂盒(湖南艾科瑞生物工程有限公司)进行实时荧光定量PCR(RT-PCR)检测。RT-PCR体系由5 μL SYBR Green Pro Taq HS Premix、2 μL cDNA、2.2 μL无RNA酶的水和0.4 μL引物对组成,总体积为10 μL。RT-PCR程序包括95 ℃ 30 s 1个循环,95 ℃ 5 s 40个循环,60 ℃ 30 s。检测空肠抗氧化和肠道形态相关基因[闭锁小带蛋白-1(ZO-1)、封闭蛋白(Occludin)、SOD1、SOD2、核因子E2相关因子2(nuclear factor E2 related factor 2,NRF2)]mRNA表达。以甘油醛-3-磷酸脱氢酶(glyceraldehyde-3-phosphate dehydrogenase,GAPDH)为内参基因,按照2-ΔΔCt的计算方法计算各目的基因的mRNA相对表达水平。RT-PCR引物序列如表4所示。
表4 RT-PCR引物序列

Table 4 Primer sequence of RT-PCR

基因
Genes
序列
Sequence (5'—3')
产物大小
Fragment size/bp
核因子E2相关因子NRF2 F:GAAAGCCCAGTCTTCATTGC
R:TTGGAACCGTGCTAGTCTCA
121
封闭蛋白Occludin F:GCCTCATCGAGTTCGCTTAC
R:CACGGACCACACTGTCAATC
105
闭锁小带蛋白-1 ZO-1 F:GTATCCTGCCGAGACTGCTC
R:TAGCAGGGACTCCAAACCAC
134
超氧化物歧化酶1 SOD1 F:ACATGGGCAATGTGACTG
R:CACAGCATTTCCCGTCT
195
超氧化物歧化酶2 SOD2 F:GGCCTACGTGAACAACCTGA
R:TGATTGATGTGGCCTCCACC
126
甘油醛-3-磷酸脱氢酶GAPDH F:ACTCACTCTTCTACCTTTGATGCT
R:TGTTGCTGTAGCCAAATTCA
123

1.5.6 结肠微生物16S rRNA基因扩增子测序

使用正向引物338F(5'-ACTCCTACGGAGGCAGCA-3')和反向引物806R(5'-GGACTACHVGGGTWTCTAAT-3')对细菌16S rRNA基因V3~V4区域进行PCR扩增。将样品特异性7-bp条形码并入引物中用于多重测序。PCR组分包含5 μL buffer(5×)、0.25 μL Fast pfuDNA聚合酶(5 U/μL)、2 μL(2.5 mmol/L) dNTP、1 μL(10 μmol/L)正向和反向引物、1 μL DNA模板和14.75 μL ddH2O。热循环包括在98 ℃下初始变性5 min,25个循环,98 ℃下变性30 s,53 ℃下退火30 s,72 ℃下延伸45 s,最后在72 ℃下延伸5 min。PCR扩增子用Vazyme VAHTSTM DNA Clean Beads(南京诺唯赞生物科技有限公司)纯化,并使用Quanti TPico Greends DNA检测试剂盒(Invitrogen公司,美国)定量。在单个定量步骤后,等量汇集扩增子,并在上海派森诺生物技术有限公司使用Illumina Nova Seq平台和NovaSeq 6000SP试剂盒(500个周期)进行双端2×250 bp测序。

1.6 数据分析

所有试验数据均采用SPSS 26.0软件进行单因素方差分析(one-way ANOVA),然后进行Duncan氏法多重比较检验。结果用平均值±标准差表示,P<0.05表示差异显著。使用GraphPad Prism 8.0软件绘制图形。

2 结果

2.1 发酵枳实残渣对仔猪生长性能的影响

表5所示,与CON组相比,8%FF组的ADG和ADFI显著提高(P<0.05)。各组之间末重和F/G无显著差异(P>0.05)。
表5 发酵枳实残渣对仔猪生长性能的影响

Table 5 Effects of fermented fructus aurantii immaturus residue on growth performance of piglets

项目
Items
组别Groups P
P-value
CON 4%FF 8%FF 12%FF
初重Initial weight/kg 7.66±0.15 7.68±0.19 7.66±0.24 7.62±0.09 0.10
末重Final weight/kg 21.13±0.49 21.33±0.50 21.76±0.50 20.48±0.34 0.29
平均日增重ADG/(g/d) 449.97±8.57bc 482.73±13.23ab 497.37±12.13a 446.85±11.35c <0.01
平均日采食量ADFI/(g/d) 873.13±24.34b 850.89±20.33b 967.29±23.30a 885.70±29.41b 0.01
料重比F/G 1.99±0.05 1.90±0.02 1.89±0.03 1.99±0.07 0.26

同行数据肩标不同小写字母表示差异显著(P<0.05),相同或无字母表示差异不显著(P>0.05)。下表同。

In the same row, values with different small letter superscripts mean significant difference (P<0.05), while with the same or no letter superscripts mean no significant difference (P>0.05). The same as below.

2.2 发酵枳实残渣对仔猪血清生化、抗氧化和免疫指标的影响

表6所示,与CON组相比,8%FF、12%FF组的血清TP含量显著提高(P<0.05),4%FF组的血清中GLU含量显著降低(P<0.05)。各组之间血清ALB、UN、CREA、TBIL含量均无显著差异(P>0.05)。与CON组相比,4%FF、8%FF、12%FF组的血清T-AOC显著提高(P<0.05),8%FF、12%FF组的血清GSH-Px活性显著提高(P<0.05),8%FF组的血清SOD活性显著提高(P<0.05),4%FF和8%FF组的血清CAT活性显著提高(P<0.05),4%FF和8%FF组的血清MDA含量显著降低(P<0.05)。与CON组相比,4%FF和8%FF组的血清IgA和IgG含量显著提高(P<0.05),8%FF组的血清IgM含量显著提高(P<0.05)。
表6 发酵枳实残渣对仔猪血清生化、抗氧化和免疫指标的影响

Table 6 Effects of fermented fructus aurantii immaturus residue on serum biochemical, antioxidant and immune indices of piglets

项目
Items
组别Groups P
P-value
CON 4%FF 8%FF 12%FF
总蛋白TP/(g/L) 48.40±0.49c 49.27±0.84bc 51.22±0.19a 50.34±0.72ab 0.02
白蛋白ALB/(g/L) 32.13±0.94 32.70±0.32 34.70±1.05 34.24±0.47 0.26
尿素氮UN/(mmol/L) 2.46±0.08 2.24±0.23 2.35±0.20 2.34±0.18 0.87
肌酐CREA/(μmol/L) 86.67±1.68 82.57±3.22 81.29±1.31 82.71±2.31 0.38
葡萄糖GLU/(mmol/L) 5.77±0.10a 5.23±0.15b 5.77±0.11a 5.73±0.14a 0.01
总胆红素TBIL/(μmol/L) 1.53±0.07 1.48±0.09 1.24±0.08 1.25±0.13 0.09
总抗氧化能力T-AOC/(U/mL) 9.14±0.62c 16.36±1.15b 23.19±1.16a 21.61±1.29a <0.01
谷胱甘肽过氧化物酶GSH-Px/(U/mL) 124.35±3.16b 139.14±5.76ab 146.87±5.92a 141.87±5.60a 0.03
超氧化物歧化酶SOD/(U/mL) 132.96±1.27b 146.86±4.84ab 162.42±8.28a 136.83±6.13b <0.01
过氧化氢酶CAT/(U/mL) 10.54±0.37b 12.28±0.56a 12.86±0.68a 11.82±0.39ab 0.03
丙二醛MDA/(nmol/mL) 9.06±0.37a 7.31±0.50bc 6.10±0.39c 8.19±0.44ab <0.01
免疫球蛋白A IgA/(μg/mL) 41.63±2.31b 53.61±2.98a 56.37±3.54a 49.31±3.46ab 0.01
免疫球蛋白G IgG/(mg/mL) 10.87±0.68b 14.07±0.92a 15.05±0.44a 14.78±0.92a <0.01
免疫球蛋白M IgM/(μg/mL) 118.39±5.18b 125.43±6.91b 149.69±6.98a 121.48±3.99b <0.01

2.3 发酵枳实残渣对仔猪空肠组织形态的影响

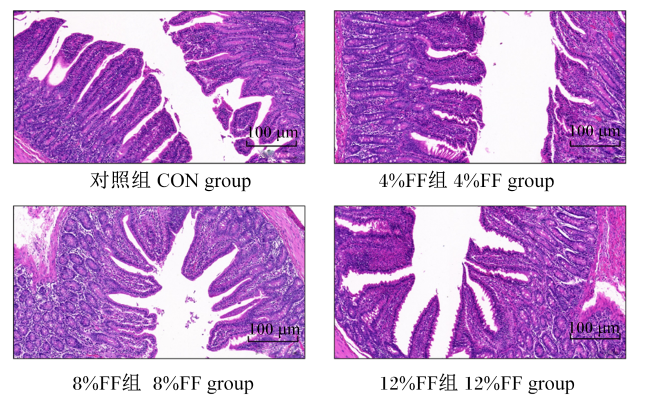
表7所示,与CON组相比,8%FF组的空肠绒毛高度、杯状细胞数量和V/C显著提高(P<0.05),空肠隐窝深度显著降低(P<0.05)。如图1所示,空肠组织切片HE染色显示CON组有少量肠绒毛断裂,其他各组空肠绒毛与肠道形态完整。
表7 发酵枳实残渣对仔猪空肠组织形态的影响

Table 7 Effects of fermented fructus aurantii immaturus residue on jejunal tissue morphology of piglets

项目
Items
组别Groups P
P-value
CON 4%FF 8%FF 12%FF
绒毛高度Villus height/μm 316.54±7.40b 334.95±11.17ab 361.62±18.73a 321.21±15.47ab <0.01
隐窝深度Crypt depth/μm 164.53±2.96a 152.79±3.00b 135.67±3.45c 152.75±3.63b <0.01
绒毛高度/隐窝深度V/C 1.93±0.06b 2.20±0.11b 2.68±0.17a 2.10±0.09b <0.01
杯状细胞数量Goblet cell number/个 22.78±1.64b 22.33±0.88b 27.42±1.41a 22.33±1.00b 0.03
图1 发酵枳实残渣对仔猪空肠组织形态的影响

Fig.1 Effects of fermented fructus aurantii immaturus residue on jejunal tissue morphology of piglets (50×)

2.4 发酵枳实残渣对仔猪空肠抗氧化和肠道形态相关基因mRNA表达的影响

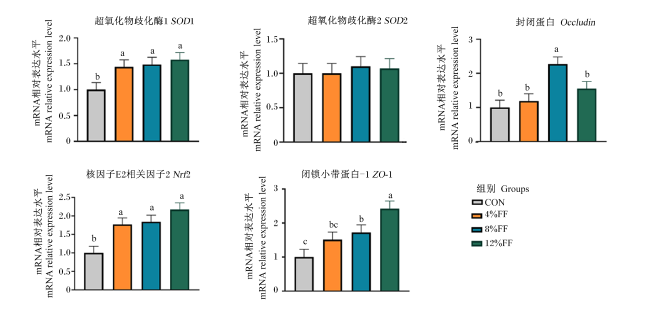
图2所示,与CON组相比,4%FF、8%FF和12%FF组的空肠SOD1和Nrf2的mRNA相对表达水平显著提高(P<0.05),8%FF组的空肠Occludin的mRNA相对表达水平显著提高(P<0.05),8%FF和12%FF组的空肠ZO-1的mRNA相对表达水平显著提高(P<0.05)。
图2 发酵枳实残渣对仔猪空肠抗氧化和肠道形态相关基因mRNA表达的影响

数据柱标相同小写字母或无字母表示差异不显著(P>0.05),不同小写字母表示差异显著(P<0.05)。下图同。

Fig.2 Effects of fermented fructus aurantii immaturus residue on mRNA expression of antioxidant and intestinal morphology related genes in jejunum of piglets

Value columns with the same small letters or no letters mean no significant difference (P>0.05), while with different small letters mean significant difference (P<0.05). The same as below.

2.5 发酵枳实残渣对仔猪结肠微生物多样性的影响

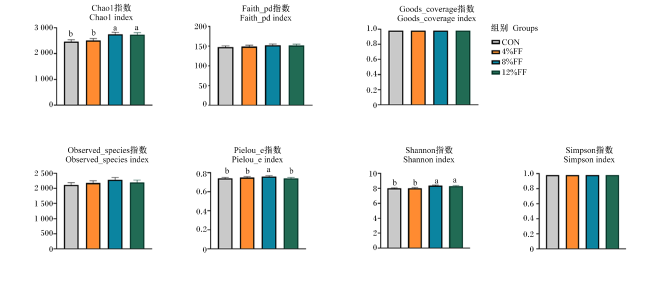
图3所示,与CON和4%FF组相比,8%FF和12%FF组的结肠微生物Chao1和Shannon指数显著提高(P<0.05);与CON组相比,8%FF组的结肠微生物Pielou_e指数显著提高(P<0.05)。
图3 发酵枳实残渣对仔猪结肠微生物α-多样性的影响

Fig.3 Effects of fermented fructus aurantii immaturus residue on colonic microbe α-diversity of piglets

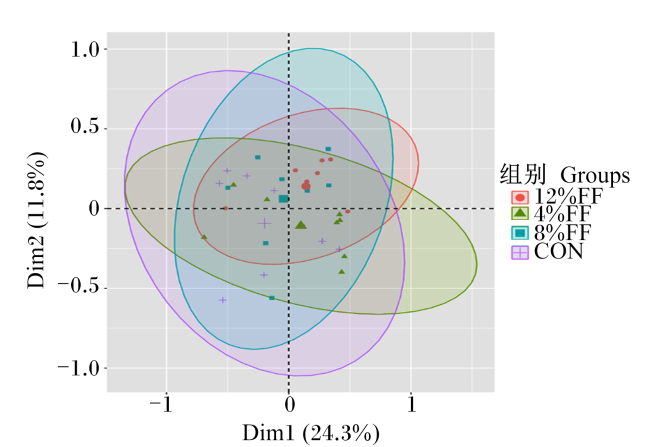
图4所示,主成分分析(PCA)显示,4%FF、8%FF和12%FF组的结肠微生物与CON组相比没有明显分离。
图4 发酵枳实残渣对仔猪结肠微生物β-多样性的影响

Dim:维度 dimension。

Fig.4 Effects of fermented fructus aurantii immaturus residue on colonic microbe β-diversity of piglets

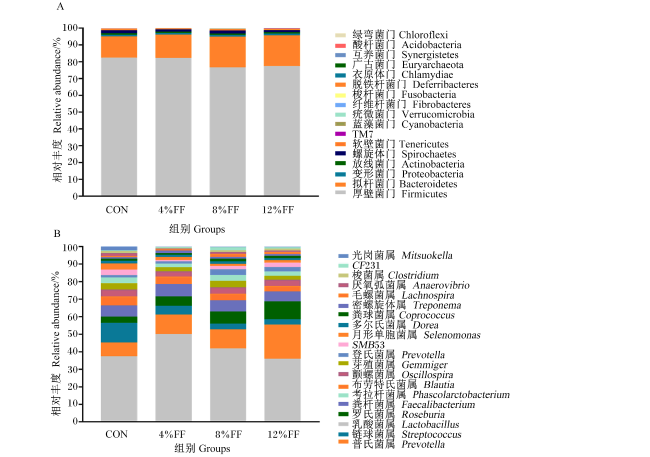
图5表8所示,在门水平上,各组优势菌群为厚壁菌门(Firmicutes)和拟杆菌门(Bacteroidetes);与CON组相比,8%FF和12%FF组的结肠Bacteroidetes相对丰度显著提高(P<0.05),结肠Firmicutes相对丰度显著降低(P<0.05)。在属水平上,各组优势菌群为乳杆菌属(Lactobacillus)和普氏菌属(Prevotella);与CON组相比,4%FF和8%FF组的结肠Lactobacillus相对丰度显著提高(P<0.05),12%FF组的结肠Prevotella相对丰度显著提高(P<0.05),4%FF、8%FF和12%FF组的结肠链球菌属(Streptococcus)相对丰度显著降低(P<0.05)。
图5 发酵枳实残渣对仔猪结肠微生物门(A)和属水平(B)优势菌群分布的影响

Fig.5 Effects of fermented fructus aurantii immaturus residue on distribution of dominant microflora at phylum (A) and genus levels (B) in colonic microbe of piglets

表8 发酵枳实残渣对仔猪结肠微生物门(A)和属水平(B)差异菌群的影响

Table 8 Effects of fermented fructus aurantii immaturus residue on differential microflora at phylum (A) and genus levels (B) in colonic microbe of piglets%

项目
Items
组别Groups P
P-value
CON 4%FF 8%FF 12%FF
厚壁菌门Firmicutes 82.52±1.56a 82.34±1.53a 76.66±0.91b 77.48±1.49b <0.01
拟杆菌门Bacteroidetes 12.65±1.30b 13.92±1.36ab 18.32±1.56a 18.31±1.87a 0.02
乳杆菌属Lactobacillus 36.43±3.99b 47.87±2.17a 46.05±2.86a 37.33±2.41b 0.02
普氏菌属Prevotella 8.07±1.28b 10.28±1.31b 11.09±0.99b 16.85±1.80a <0.01
链球菌属Streptococcus 11.39±0.95a 6.04±1.38b 3.61±0.52b 3.49±0.46b <0.01

3 讨论

枳实中含有辛弗林等生物碱类、橙皮苷等黄酮类、柠檬烯等挥发油类主要有效成分,对胃肠道功能有显著改善作用[11]。枳实的3个主化合物分别为橙皮苷、川陈皮素和桔皮素。饲粮中添加8%的发酵枳实残渣能显著提高仔猪的ADFI和ADG,而添加4%和12%的发酵枳实残渣对仔猪的ADFI和ADG没有显著改善效果,表明饲粮中适量使用发酵枳实残渣能改善仔猪的食欲,这可能与枳实中含有橙皮苷成分有关。研究发现,橙皮苷能够增加胃排空率和小肠推进率,增加胃动素的释放,从而改善功能性消化不良,促进胃肠动力[12]。枳实黄酮类化合物通过提高小肠推进速率促进胃肠运动[13],发酵枳实残渣进入断猪肠道后加速小肠对其他营养物质的消化吸收,进而提高ADG。推测饲粮中添加8%的发酵枳实残渣改善仔猪生长性能,可能与枳实中的橙皮苷和黄酮类化合物有关。
血清生化指标可反映机体营养代谢水平及健康状况[14],在本试验中,饲粮中添加8%和12%的发酵枳实残渣显著提高血清TP含量,可能是在枳实生物活性成分的作用下,仔猪机体新陈代谢得到提高,但具体发挥作用的活性成分还需要进一步研究;饲粮中添加4%的发酵枳实残渣显著降低了血清GLU含量,说明发酵枳实残渣降低了机体的能量代谢水平。IgA、IgG和IgM是判断机体免疫功能的重要指标,主要由B淋巴细胞分泌,对机体体液免疫有十分重要的作用[15]。本试验中,饲粮中添加8%的发酵枳实残渣显著提高了血清IgA、IgG和IgM含量,表明发酵枳实残渣能提高仔猪的机体免疫性能。
枳实中的黄酮类成分中的柚皮苷、橙皮苷、橙皮素等均具有抗氧化作用。焦士蓉等[16]研究表明,枳实提取物具有较强的清除自由基及抑制脂质过氧化的能力。用枳实提取物对糖尿病小鼠进行治疗,发现小鼠的肾脏抗氧化酶活性增强,并有一定的降血糖作用。用枳实水提物给大鼠灌服可通过降低大鼠的血液内毒素和肿瘤坏死因子-α(TNF-α)含量发挥抗氧化作用[17]。本试验结果显示,饲粮中添加8%的发酵枳实残渣显著提高了仔猪血清GSH-Px、SOD、CAT活性和T-AOC,同时显著降低了血清MDA含量,表明发酵枳实残渣能改善机体的抗氧化能力。发酵枳实残渣不仅能通过增强抗氧化酶活性来增强机体抗氧化能力,还通过调控抗氧化基因mRNA的表达水平来发挥抗氧化作用。本研究结果显示,饲粮中添加4%、8%和12%的发酵枳实残渣能显著上调空肠SOD1和Nrf2的mRNA相对表达水平。发酵枳实残渣的抗氧化作用主要与其含有的生物活性物质有关,除了黄酮类化合物外,其中的酚类化合物也具有较强的抗氧化能力,但目前关于发酵枳实残渣中酚类化合物的特征及抗氧化能力的报道较少[18]
小肠黏膜形态结构的完整性是保证动物维持肠道正常生理活动的基础[19]。小肠绒毛的作用主要是增加小肠的吸收面积并起到过滤物质的作用[20]。肠隐窝深度主要反映肠上皮细胞的成熟率,隐窝变浅表明上皮细胞成熟率增加,分泌功能增强[21]。V/C反映小肠的功能状态,绒毛长度变短,隐窝深度变深即V/C下降,意味着绒毛吸收细胞减少,分泌细胞增多,肠内膜面积减少,小肠消化吸收功能下降,常伴随腹泻的发生[22]。杯状细胞分泌的黏蛋白与柱状细胞分泌的复合糖蛋白一起形成肠道上皮细胞的表面细胞衣。该细胞衣的糖蛋白与细胞膜的蛋白质与脂质紧密结合,作为肠道上皮的重要物理屏障,可以阻挡致病微生物与有害物质的侵袭,防止致病源对机体造成伤害[23]。在本试验中,饲粮中添加8%的发酵枳实残渣显著提高了空肠绒毛高度、杯状细胞数量以及V/C,显著降低了隐窝深度,提示发酵枳实残渣有利于仔猪肠道形态的改善。此外,V/C的提高增加了肠黏膜有效吸收面积,加速小肠对营养物质的吸收和利用,最终提高仔猪的ADG。
动物在健康状态下,其肠道微生物处于动态平衡状态,这些长期定植在动物肠道的微生物作为肠道内环境的重要组成部分而存在[24]。肠道微生物菌群通过定植肠道增加肠道抵抗力,帮助机体防御病原菌的入侵[25],也可通过增强机体对病原菌的免疫应答和阻止病原菌在肠道的附着,帮助机体免受外来病原菌感染[26]。本试验结果显示,肠道微生物的结构因添加发酵枳实残渣而发生了改变,添加发酵枳实残渣组的肠道微生物多样性明显高于对照组,枳实的有效成分柚皮苷具有一定的抑菌作用[19,27],推测发酵枳实通过抑制有害菌的同时促进有益菌的增加。
本试验结果显示,在门水平上,Bacteroidetes和Firmicutes是优势菌群。值得注意的是,Bacteroidetes和Firmicutes都是发酵多糖的主力军,当肠道内Firmicutes/Bacteroidetes(F/B)比例较高时,宿主摄取食物中能量的能力会加强,体内脂肪的贮存也会加剧[28]。郭秀兰[29]也进一步证实猪脂肪沉积与肠道的Bacteroidetes及F/B比例相关,他们认为调控肠道微生物可作为控制猪脂肪沉积的途径之一。在本试验中,随着发酵枳实残渣添加水平的增加,Bacteroidetes相对丰度和F/B比例增加,进一步证实仔猪ADG增加的原因。此外,我们推测发酵枳实残渣还有利于仔猪体内脂肪的沉积;在属水平上,饲粮中添加发酵枳实残渣提高了结肠Lactobacillus相对丰度,进而帮助仔猪激活机体建立健康的肠道环境以防御病原体入侵[30]。研究发现,以Prevotella为主的肠道微生物的ADFI更高,富含Prevotella的肠道微生物群可以增强猪的生长性能[31]。本研究中,发酵枳实残渣可能通过提高Prevotella的相对丰度以增加仔猪采食量,从而改善生长性能。Streptococcus是一种新兴的人畜共患病原体,可引起败血症、肺炎、心内膜炎、关节炎和脑膜炎,并伴有不可逆的后遗症[32]。Benzaid等[27]在研究中证明枳实挥发油能抑制Streptococcus的生长,降解其成熟的生物膜;在本试验中,饲粮中添加发酵枳实残渣显著降低了结肠Streptococcus的相对丰度,预防炎症的发生,这可能是枳实中的挥发油起着关键作用。综上所述,发酵枳实残渣可能通过改善肠道微生物的组成促进仔猪的肠道健康。

4 结论

饲粮中添加8%发酵枳实残渣对仔猪生长性能无负面影响,且能改善其抗氧化能力,并通过丰富肠道微生物多样性促进仔猪的肠道健康,为发酵枳实残渣在养猪生产中的应用提供数据支撑。
[1]
杨玉环, 张灵煜, 郭秋平, 等. 枳实、枳壳的生物活性成分及其应用研究进展[J]. 食品与药品, 2021, 23(5):476-484.

YANG Y H, ZHANG L Y, GUO Q P, et al. Bioactive components of fructus aurantii immaturus and fructus aurantii and their application[J]. Food and Drug, 2021, 23(5):476-484. (in Chinese)

[2]
张霄潇, 李正勇, 马玉玲, 等. 中药枳实的研究进展[J]. 中国中药杂志, 2015, 40(2):185-190.

ZHANG X X, LI Z Y, MA Y L, et al. Progress in research of traditional Chinese medicine Citrus aurantium[J]. China Journal of Chinese Materia Medica, 2015, 40(2):185-190. (in Chinese)

[3]
胡源祥, 陈海芳, 宋玉鹏, 等. 枳实及其主要活性成分促进脾虚模型大鼠胃肠运动的机制研究[J]. 中国药房, 2017, 28(13):1747-1750.

HU Y X, Chen H F, SONG Y P, et al. Study on the mechanism of fructus aurantii immaturus and its main active ingredients in promoting gastrointestinal motility of model rats with spleen deficiency[J]. China Pharmacy, 2017, 28(13):1747-1750. (in Chinese)

[4]
TAKASE H, YAMAMOTO K, HIRANO H, et al. Pharmacological profile of gastric mucosal protection by marmin and nobiletin from a traditional herbal medicine,aurantii fructus immaturus[J]. Japanese Journal of Pharmacology, 1994, 66(1):139-147.

[5]
舒一崧. 橘属中药的药效物质基础及枳实对APAP诱导的肝损伤的保护作用研究[D]. 硕士学位论文. 北京: 北京中医药大学, 2018.

SHU Y S. Study on the pharmacodynamic material basis of tangerine and the protective effect of trifoliate on APAP-induced liver injury[D]. Master’s Thesis. Beijing: Beijing University of Chinese Medicine, 2018. (in Chinese)

[6]
焦士蓉, 黄承钰, 王波, 等. 枳实提取物对实验性糖尿病小鼠肝脏抗氧化防御功能的影响[J]. 卫生研究, 2007, 36(6):689-692.

JIAO S R, HUANG C Y, WANG B, et al. Effects of Citrus aurantium extract on liver antioxidant defense function in experimental diabetic mouse[J]. Journal of Hygiene Research, 2007, 36(6):689-692. (in Chinese)

[7]
赵志超, 图门巴雅尔. 中草药提取残渣综合利用研究进展[J]. 畜牧与饲料科学, 2019, 40(2):47-52.

ZHAO Z C, TUMEN B Y E. Research progress on comprehensive utilization of extracting residues from traditional Chinese medicine[J]. Animal Husbandry and Feed Science, 2019, 40(2):47-52. (in Chinese)

[8]
李春荣. 发酵柑橘渣对生长育肥猪生产性能、抗氧化能力、免疫力和肉质的影响[D]. 硕士学位论文. 重庆: 西南大学, 2022.

LI C R. Effects of fermented citrus pulp on production performance,antioxidant capacity,immunity and meat quality of growing-finishing pigs[D]. Master’s Thesis. Chongqing: Southwest University, 2022. (in Chinese)

[9]
张兆兰. 能量饲料和蛋白质饲料中消化能(猪)的计算[J]. 河北畜牧兽医, 1993, 9(2):92.

ZHANG Z L. Calculation of digestible energy (pig) in energy feed and protein feed[J]. Hebei Animal Husbandry and Veterinary Science, 1993, 9(2):92. (in Chinese)

[10]
NOSWORTHY M G, DODGE M E, BERTOLO R F, et al. Enterally delivered dipeptides improve small intestinal inflammatory status in a piglet model of intestinal resection[J]. Clinical Nutrition, 2016, 35(4):852-858.

DOI PMID

[11]
谭舒舒, 陈海芳, 宋玉鹏, 等. 枳壳及其主要活性成分对脾虚模型大鼠血清胃泌素、血浆乙酰胆碱、胃动素、P物质和血管活性肠肽的影响[J]. 时珍国医国药, 2017, 28(5):1037-1040.

TAN S S, CHEN H F, SONG Y P, et al. Effects of fructus aurantii and its main active ingredients on serum gastrin,plasma acetylcholine,motilin,substance P and vasoactive intestinal peptide in rats with spleen deficiency model[J]. Lishizhen Medicine and Materia Medica Research, 2017, 28(5):1037-1040. (in Chinese)

[12]
黄爱华, 迟玉广, 曾元儿, 等. 枳实黄酮对功能性消化不良大鼠胃肠动力的影响[J]. 中药新药与临床药理, 2012, 23(6):612-615.

HUANG A H, CHI Y G, ZENG Y E, et al. Influence of fructus aurantii immaturus flavonoids on gastrointestinal motility in rats with functional dyspepsia[J]. Traditional Chinese Drug Research and Clinical Pharmacology, 2012, 23(6):612-615. (in Chinese)

[13]
TAN W X, LI Y, WANG Y, et al. Anti-coagulative and gastrointestinal motility regulative activities of fructus aurantii immaturus and its effective fractions[J]. Biomedicine & Pharmacotherapy, 2017, 90:244-252.

DOI

[14]
MADRID J, VILLODRE C, VALERA L, et al. Effect of crude glycerin on feed manufacturing,growth performance,plasma metabolites,and nutrient digestibility of growing-finishing pigs[J]. Journal of Animal Science, 2013, 91(8):3788-3795.

DOI

[15]
邹士海, 吴颖. 中草药添加剂对母猪及仔猪免疫力的影响[J]. 浙江畜牧兽医, 2021, 46(4):1-3.

ZOU S H, WU Y. The effect of Chinese herbal medicine additive on immunity of sows and their piglets[J]. Zhejiang Journal Animal Science and Veterinary Medicine, 2021, 46(4):1-3. (in Chinese)

[16]
焦士蓉, 马力, 黄承钰, 等. 枳实提取物的体外抗氧化作用研究[J]. 中药材, 2008, 31(1):113-116.

JIAO S R, MA L, HUANG C Y, et al. Study on the antioxidant effect of extracts from trifoliate aurantium in vitro[J]. Journal of Chinese Medicinal Materials, 2008, 31(1):113-116. (in Chinese)

[17]
LIU X Y, FAN M L, WANG H Y, et al. Metabolic profile and underlying improved bio-activity of fructus aurantii immaturus by human intestinal bacteria[J]. Food & Function, 2017, 8(6):2193-2201.

[18]
FERREIRA S S, SILVA A M, NUNES F M. Citrus reticulata Blanco peels as a source of antioxidant and anti-proliferative phenolic compounds[J]. Industrial Crops and Products, 2018, 111:141-148.

DOI

[19]
HOUSHMAND M, AZHAR K, ZULKIFLI I, et al. Effects of non-antibiotic feed additives on performance,immunity and intestinal morphology of broilers fed different levels of protein[J]. South African Journal of Animal Science, 2012, 42(1):22-32.

[20]
王永超. 肠膜蛋白粉和发酵豆粕替代鱼粉对断奶仔猪作用效果的研究[D]. 硕士学位论文. 洛阳: 河南科技大学, 2015.

WANG Y C. Effect of intestinal membrane protein and fermented soybean meal replacing fish meal on weaned piglets[D]. Master’s Thesis. Luoyang: Henan University of Science and Technology, 2015. (in Chinese)

[21]
YANG H S, XIONG X, WANG X C, et al. Effects of weaning on intestinal upper villus epithelial cells of piglets[J]. PLoS One, 2016, 11(3):e0150216.

DOI

[22]
SEGAWA S C, FUJIYA M, KONISHI H, et al. Probiotic-derived polyphosphate enhances the epithelial barrier function and maintains intestinal homeostasis through integrin-p38 MAPK pathway[J]. PLoS One, 2011, 6(8):e23278.

DOI

[23]
王继凤. 丁酸钠对断奶仔猪肠黏膜结构及黏膜免疫相关细胞影响的研究[D]. 硕士学位论文. 北京: 中国农业大学, 2005.

WANG J F. Studies on effect of sodium butyrate on the structure of gut mucous and mucosal immunity-associated cell in weaned piglet[D]. Master’s Thesis. Beijing: China Agricultural University, 2005. (in Chinese)

[24]
SCHIFFRIN E J, BLUM S. Interactions between the microbiota and the intestinal mucosa[J]. European Journal of Clinical Nutrition, 2002, 56(Suppl.3):S60-S64.

DOI

[25]
MAY K D, WELLS J E, MAXWELL C V, et al. Granulated lysozyme as an alternative to antibiotics improves growth performance and small intestinal morphology of 10-day-old pigs[J]. Journal of Animal Science, 2012, 90(4):1118-1125.

DOI PMID

[26]
INOUE R, TSUKAHARA T, NAKANISHI N, et al. Development of the intestinal microbiota in the piglet[J]. The Journal of General and Applied Microbiology, 2005, 51(4):257-265.

DOI

[27]
NIDHI P, ROLTA R, KUMAR V, et al. Synergistic potential of Citrus aurantium L. essential oil with antibiotics against Candida albicans[J]. Journal of Ethnopharmacology, 2020, 262:113135.

DOI

[28]
LEY R E, BÄCKHED F, TURNBAUGH P, et al. Obesity alters gut microbial ecology[J]. Proceedings of the National Academy of Sciences of the United States of America, 2005, 102(31):11070-11075.

DOI PMID

[29]
郭秀兰. 猪肠道硬壁菌门和拟杆菌门数量的检测及其相对丰度与脂肪沉积的相关性研究[D]. 博士学位论文. 雅安: 四川农业大学, 2009.

GUO X L. Detection of firmicutes and bacteroidetes in the pig gut and the correlation between their abundance and fat deposit[D]. Ph.D.Thesis. Ya’an: Sichuan Agricultural University, 2009. (in Chinese)

[30]
YANG J J, QIAN K, WANG C L, et al. Roles of probiotic lactobacilli inclusion in helping piglets establish healthy intestinal inter-environment for pathogen defense[J]. Probiotics and Antimicrobial Proteins, 2018, 10(2):243-250.

DOI PMID

[31]
MACH N, BERRI M, ESTELLÉ J, et al. Early-life establishment of the swine gut microbiome and impact on host phenotypes[J]. Environmental Microbiology Reports, 2015, 7(3):554-569.

DOI PMID

[32]
HAAS B, GRENIER D. Understanding the virulence of Streptococcus suis:a veterinary,medical,and economic challenge[J]. Medecine et Maladies Infectieuses, 2018, 48(3):159-166.

DOI

文章导航

/