研究论文

混合益生菌对大口黑鲈生长性能、肉品质及肠道健康的影响

  • 周秀珍 , 1 ,
  • 刘滔 2 ,
  • 张毅 1 ,
  • 王扬 3 ,
  • 赵敏洁 4 ,
  • 王旭堂 5 ,
  • 黄菊 , 1, * ,
  • 冯凤琴 , 4, *
展开
  • 1 浙江海洋大学食品与药学学院,舟山 316022
  • 2 湘湖实验室,杭州 311203
  • 3 浙江省水产技术推广总站,杭州 311110
  • 4 浙江大学生物系统工程与食品科学学院,杭州 310058
  • 5 杭州龙宇生物科技有限公司,杭州 310030
*黄菊,副教授,硕士生导师,E-mail: ;
冯凤琴,教授,博士生导师,E-mail:

周秀珍(1998—),女,内蒙古乌兰察布人,硕士研究生,研究方向为食品化学。E-mail:

Copy editor: 武海龙

收稿日期: 2024-01-18

  网络出版日期: 2024-07-09

基金资助

浙江省科技计划项目—多营养层级高效水产养殖技术(2022C02040)

Effects of Mixed Probiotics on Growth Performance, Meat Quality and Intestinal Health of Largemouth Bass (Micropterus salmoides)

  • ZHOU Xiuzhen , 1 ,
  • LIU Tao 2 ,
  • ZHANG Yi 1 ,
  • WANG Yang 3 ,
  • ZHAO Minjie 4 ,
  • WANG Xutang 5 ,
  • HUANG Ju , 1, * ,
  • FENG Fengqin , 4, *
Expand
  • 1 College of Food and Pharmacy, Zhejiang Ocean University, Zhoushan 316022, China
  • 2 Xianghu Laboratory, Hangzhou 311203, China
  • 3 Zhejiang Aquatic Product Technology Promotion General Station, Hangzhou 311110, China
  • 4 College of Biosystems Engineering and Food Science, Zhejiang University, Hangzhou 310058, China
  • 5 Hangzhou Longyu Bio-Technology Co., Ltd., Hangzhou 310030, China
*HUANG Ju, associate professor, E-mail: ;
FENG Fengqin, professor, E-mail:

Received date: 2024-01-18

  Online published: 2024-07-09

摘要

本试验旨在探究混合益生菌(凝结芽孢杆菌、植物乳杆菌、鼠李糖乳杆菌和嗜酸乳杆菌,活菌数≥1.75×10⁹ CFU/g)对大口黑鲈生长性能、肉品质及肠道健康的影响。选择990尾初始体重为(36.17±1.52) g大口黑鲈,随机分为3组,每组3个重复,每个重复110尾。各组分别饲喂基础饲料中添加0(对照组,CON组)、0.1%(MP-0.1%组)和1.0%(MP-1.0%组)的混合益生菌。试验期130 d。结果表明:1)各组之间生长性能和形体指标无显著差异(P>0.05)。2)与CON组相比,MP-0.1%和MP-1.0%组的肌肉纤维直径显著降低(P<0.05),MP-1.0%组的肌肉密度显著升高(P<0.05)。3)与CON组相比,MP-1.0%组的肌肉硬度、胶黏性和咀嚼性显著升高(P<0.05)。4)与CON组相比,MP-1.0%组的肌肉水分含量显著降低(P<0.05),肌肉粗蛋白质、风味氨基酸(鲜味氨基酸、甜味氨基酸)、多不饱和脂肪酸、omega-3脂肪酸及omega-6脂肪酸含量显著升高(P<0.05);MP-0.1%组的肌肉多不饱和脂肪酸和omega-3脂肪酸含量显著升高(P<0.05),而肌肉单不饱和脂肪酸含量显著下降(P<0.05)。5)与CON组相比,MP-0.1%和MP-1.0%组的肌肉中土臭素和2-甲基异莰醇含量均显著降低(P<0.05)。6)与CON组相比,MP-1.0%组的胃蛋白酶和胰蛋白酶活性均显著升高(P<0.05)。7)与CON组相比,MP-0.1%组的肠道绒毛宽度显著升高(P<0.05)。8)与CON组相比,MP-1.0%组的肠道异戊酸和总酸含量显著升高(P<0.05)。9)3组之间的肠道鲸杆菌属(Cetobacterium)和消化链球菌属(Peptostreptococcus)相对丰度具有显著差异(P<0.05),且MP-0.1%和MP-1.0%组的肠道菌群相似度更高,明显不同于CON组。由此可见,饲料中添加混合益生菌可改善大口黑鲈的肉品质及肠道健康。本试验条件下,大口黑鲈饲料中混合益生菌的适宜添加水平为1.0%。

本文引用格式

周秀珍 , 刘滔 , 张毅 , 王扬 , 赵敏洁 , 王旭堂 , 黄菊 , 冯凤琴 . 混合益生菌对大口黑鲈生长性能、肉品质及肠道健康的影响[J]. 动物营养学报, 2024 , 36(7) : 4588 -4609 . DOI: 10.12418/CJAN2024.394

Abstract

The aim of this experiment was to investigate the effects of mixed probiotics (Bacillus coagulans, Lactobacillus plantarum, Lactobacillus rhamnosus and Lactobacillus acidophilus, and viable count ≥1.75×10⁹ CFU/g) on the growth performance, meat quality and intestinal health of largemouth bass (Micropterus salmoides). A total of 990 largemouth bass with initial body weight of (36.17±1.52) g were randomly divided into 3 groups with 3 replicates in each group and 110 fish in each replicate. Fish in 3 groups were fed the basal diets supplemented with 0 (control group, CON group), 0.1% (MP-0.1% group) and 1.0% (MP-1.0% group) mixed probiotics, respectively. The experiment lasted for 130 days. The results showed as follows: 1) there were no significant differences in growth performance and shape indexes among all groups (P>0.05). 2) Compared with the CON group, the myofiber diameter of MP-0.1% and MP-1.0% groups was significantly decreased (P<0.05), and the myofiber density of MP-1.0% group was significantly increased (P<0.05). 3) Compared with the CON group, the muscle hardness, gumminess and chewiness of MP-1.0% group were significantly increased (P<0.05). 4) Compared with the CON group, the muscle moisture content of MP-1.0% group was significantly decreased (P<0.05), and the contents of crude protein, flavor amino acids (delicious amino acids and sweet amino acids), polyunsaturated fatty acids, omega-3 fatty acids and omega-6 fatty acids in muscle were significantly increased (P<0.05); the contents of polyunsaturated fatty acids and omega-3 fatty acids in muscle of MP-0.1% group were significantly increased (P<0.05), and the muscle monounsaturated fatty acids content was significantly decreased (P<0.05). 5) Compared with the CON group, the contents of geosmin and 2-methyli-soborneol in muscle of MP-0.1% and MP-1.0% groups were significantly decreased (P<0.05). 6) Compared with the CON group, the activities of pepsin and trypsin in intestine of MP-1.0% group were significantly increased (P<0.05). 7) Compared with the CON group, the intestinal villus width of MP-0.1% group was significantly increased (P<0.05). 8) Compared with the CON group, the contents of isovaleric acid and total acid in intestine were significantly increased (P<0.05). 9) The relative abundances of Cetobacterium and Peptostreptococcus in intestine had significantly different among three groups (P<0.05), and the MP-0.1% and MP-1.0% groups had more similar intestinal flora, which were different from the CON group. In conclusion, dietary mixed probiotics can improve the meat quality and intestinal health of largemouth bass. Under the conditions of this experiment, the dietary mixed probiotics appropriate supplemental level is 1.0%.

大口黑鲈(Micropterus salmoides)又称加州鲈,属硬骨鱼纲、鲈形目、太阳鱼科、黑鲈属。大口黑鲈是一种肉食性鱼类,原产于美国加利福尼亚州密西西比河水系[1],1983年首次在我国台湾成功繁育,之后在全国范围推广养殖。目前大口黑鲈的养殖主要分布在我国沿海地区,特别是广东和江浙一带[2]。大口黑鲈捕食能力好,生长速度快,抗病能力强,肉质营养丰富,味道鲜美,无肌间刺,受到养殖户和消费者的青睐。为了追求更高的经济效益,许多养殖户采取高密度养殖,导致水质和鱼病问题的频发及肉品质的下降[3]。在抗生素治疗的同时,不仅使细菌产生耐药性,造成恶性循环,同时这些化学药物通过食物链富集,也会危害人体健康[4]
目前,益生菌作为抗生素的替代产品受到了广泛的关注[5-6]。益生菌是指通过食物或水进入胃肠道的活微生物,通过调节宿主体内微生态平衡,从而促进宿主机体健康[6]。早在2008年,益生菌就被建议用在水产养殖中,并已有文章证实,益生菌对水产动物具有很好的调节作用,包括生长性能、免疫力、抗病能力、肠道微生物等[7-10]。植物乳杆菌(Lactobacillus plantarum)是一种革兰氏阳性杆菌,兼性厌氧,对胆汁酸和盐及多种抗生素具有很强的耐受性[11],并能够积极改善多种水产动物的生长性能、免疫力和抗菌能力[12-16]。凝结芽孢杆菌(Bacillus coagulans)是一种兼性厌氧菌,对酸和胆汁盐有较高的耐受,能够促进双歧杆菌等有益菌的生长繁殖,抑制有害菌增殖[17],并能提高鱼体生长性能、营养成分含量、抗氧化能力、免疫力和抗病能力,调节肠道微生物菌群[18-22]。鼠李糖乳杆菌(Lactobacillus rhamnosus)是一种革兰氏阳性益生菌,具有耐酸、耐胆汁盐、耐多种抗生素等生物学特点[23],能够提高鱼体生长性能、蛋白质消化率、营养成分含量、血清溶菌酶和超氧化物歧化酶活性、抗应激反应能力及肠道绒毛长度[24-28]
近年来,益生菌作为鱼类饲料添加剂已被广泛研究,但多数研究更多关注鱼类的生长性能、免疫和肠道微生态的调节等方面,对肉品质影响的研究甚少,然而鱼肉质量是消费者购买的主要因素之一。肉品质评价内容包括物理性质(硬度、弹性和咀嚼性等)、营养价值和风味等[29]。肉品质与鱼体肠道健康状况(消化酶活性、肠道形态、短链脂肪酸含量及微生态环境等)密不可分,肠道健康状况影响营养物质的消化吸收,从而改变鱼体生长性能和肉品质[30]。而鱼体的生长性能和形体指标反映鱼体的营养价值和健康状况,也是经济价值的重要指标。因此,本文旨在探究混合益生菌对大口黑鲈生长性能、形体指标、肉品质及肠道健康的影响,以期为混合益生菌作为饲料添加剂提供理论参考。

1 材料与方法

1.1 试验设计及饲料配制

选择990尾初始体重为(36.17±1.52) g的大口黑鲈,随机分为3组,每组3个重复,每个重复110尾。分别将质量分数为0(对照组,CON组)、0.1%(MP-0.1%组)和1.0%(MP-1.0%组)的混合益生菌添加到基础饲料中,即各组饲料中的活菌数分别为0、1.75×10⁹和1.75×10¹⁰ CFU/kg。与基础饲料充分混匀后,制成3种试验饲料,于-20 ℃条件下保存。混合益生菌由凝结芽孢杆菌、植物乳杆菌、鼠李糖乳杆菌和嗜酸乳杆菌复配而成,粉状,活菌数为1.75×10⁹ CFU/g。试验期130 d。

1.2 饲养管理

饲养试验在浙江省恒泽生态农业养殖基地进行。大口黑鲈经过2周暂养后,随即分配到9个养殖缸(直径3 m),循环水养殖,每缸110尾(养殖密度22尾/m3)。每天人工投喂饲料2次,投喂20 min后收集并记录残饵重,投喂量为体重的1%,可根据天气情况做适当调整。大口黑鲈养殖水温控制在19~35 ℃,养殖水溶氧量为(4.48±0.78) mg/L,氨氮含量为(0.41±0.78) mg/L,pH为8.18±0.12,亚硝酸盐含量为(0.14±0.02) mg/L,余氯含量为(0.07±0.02) mg/L。

1.3 样品采集

在试验第130天,对养殖缸中的鱼先禁食24 h,用丁香酚(购自上海阿拉丁生化科技有限公司)麻醉,记录每缸中存活鱼数,同时测量缸中所有鱼的体重、体长和体宽。随即从每缸中随机选取5尾鱼,解剖,测量其内脏团和肝脏质量,并收集后肠内容物置于微生物样品专用管中,用于肠道微生物测序;前肠内容物经液氮速冻后于-80 ℃保存,用于短链脂肪酸含量和消化酶活性测定;中肠放入装有4%多聚甲醛的离心管中,室温保存以备组织学检测。最后去皮,取相同位置的背肌(1.5 cm×1.5 cm×1.5 cm),放入装有4%多聚甲醛的离心管中,室温保存以备组织学检测。剩余背肌分为2部分,一部分用于质构检测,另一部分用液氮快速冷冻用于其他理化指标检测,并保存在-80 ℃冰箱中。

1.4 试验试剂和仪器

氢氧化钠、硫酸钾、硫酸、盐酸、石油醚、无水乙醚、无水乙醇均购自上海凌峰化学试剂有限公司,硫酸铜、硼酸、氯化钠均购自国药集团化学试剂有限公司,正庚烷、焦性没食子酸、三氟化硼-甲醇均购自上海麦克林生化科技股份有限公司,甲醇、乙腈均购自赛默飞世尔科技(中国)有限公司,乙二胺-N-丙基硅烷(PSA)、石墨化炭黑(C18)均购自美国Agilent Technologies公司,2-甲基异莰醇(2-methyli-soborneol,2-MIB)、土臭素(geosmin,GSM)、2-异丁基-3-甲氧基吡嗪(2-isobutyl-3-methoxypyrazine,IBMP)均购自天津阿尔塔科技有限公司,乙酸、丙酸、正丁酸、异丁酸、正戊酸、异戊酸、正己酸、2-乙基丁酸均购自上海阿拉丁生化科技股份有限公司,胃蛋白酶、胰蛋白酶试剂盒均购自南京建成生物工程研究所,QIAamp DNA Stool Mini Kit、Qiagen Gel Extraction Kit均购自德国Qiagen Gel Extraction公司,KAPA HiFi Hotstart Ready Mix PCR Kit购自美国KAPA Biosystems公司,AxyPerp DNA购自美国AXYGEN公司,UltraTM DNA Library Prep Kit for Illumina购自英国New England Biolabs公司,琼脂糖凝胶购自西班牙Biowest公司。
Stemi-508体式显微镜购自德国蔡司集团,物性分析仪购自英国Stable Micro Systems公司,电子天平购自METTLE TOLEDO仪器(上海)有限公司,DGG-9070A型电热恒温鼓风干燥箱购自上海森信实验仪器有限公司,灰化炉购自英国弗尔德集团,B-324蒸馏仪、K-435消化仪、B-811索氏提取仪均购自瑞士Buchi公司,Allegra X-12 Centrifuge台式离心机购自美国Beckman Coulter公司,全自动氨基酸分析仪购自日本日立公司,6890N气相色谱仪、DB-23122-2361色谱柱、FID检测器、6890N GC-5973 MS、HP-5MS气相色谱柱均购自美国Agilent Technologies公司,UV2006分光光度计购自日本岛津公司,MDF-U53V超低温冰箱日本Panasonic Healthcare公司,LDZF-50KB-Ⅱ高压灭菌锅购自上海申安医疗器械厂,HC-3018R高速冷冻离心机购自安徽中科中佳科学仪器有限公司,H1650-W高速离心机购自湖南湘仪实验室仪器开发有限公司,Infinite M200 Pro酶标仪购自瑞士帝肯(TECAN)集团公司,JS-680B凝胶成像仪购自上海培清科技有限公司,Mastercycler Pro PCR仪购自德国Eppendorf公司,PB-10 pH剂购自赛多利斯科学仪器有限公司,ZHJHC1112B无菌操作台购自上海智诚分析仪器制造有限公司,LightCycler480 II荧光定量PCR仪购自美国罗氏公司,DYCZ-22A电泳仪、Nanodrop 2000核酸浓度检测仪、Qubit 2.0荧光分光光度计均购自美国Thermo公司,PT-2100组织匀浆机购自瑞士Kinematica公司。

1.5 指标测定

1.5.1 生长性能和形体指标

生长性能和形体指标计算公式如下:
存活率(SR,%)=(Nt/N0)×100;
增重率(WGR,%)=(Wt-W0)/W0×100;
饲料效率(FCR)=(Wt-W0)/Df;
特定生长率(SGR,%/d)=[(lnWt-lnW0)/t]×100;
肥满度(CF,g/cm3)=(Wt/L3)×100;
脏体比(VI,%)=(Wv/Wt)×100;
肝体比(HI,%)=(WL/Wt)×100。
式中:W0WtWvWL分别为鱼体初始体重、终末体重、内脏团湿重和肝脏湿重;L为鱼体长度;t为试验天数;N0Nt分别为试验开始和试验结束时网箱中鱼的尾数;Df为摄食干重。

1.5.2 肌肉纤维指标

取大口黑鲈背部肌肉,用4%的多聚甲醛固定,然后经洗涤、脱水、浸蜡、包埋、切片、展片、脱蜡、染色、封片后,在光学显微镜下对组织切片进行观察和分析。拍照时在相同的光源下,每片大口黑鲈肌肉切片放大倍数固定为100倍,使肌肉切片全部出现在同一视野下。拍好后每张肌肉切片选取20个肌肉纤维,用ZEN 3.0软件测量并统计每个肌肉纤维的面积,并计算肌肉纤维直径(μm)。同时记录在51 μm×42 μm视野下的肌肉纤维个数,并计算肌肉纤维密度(个/μm2)。

1.5.3 肌肉质构指标

参照李温蓉等[31]的方法,取每条鱼去皮后背部两侧肌肉进行测定,每条鱼平行测定2次,每组平行30次,将鱼肉修剪成长×宽×高=1 cm×1 cm×1 cm的正方体,靠近鱼皮面朝上进行测定。采用TA.XTPlus物性测试仪,配以P6平底柱形探头,对试样进行全质构模式测试,测试设定参数如下:测前速度2 mm/s,测试速度3 mm/s,测试后速度5 mm/s,肌肉变形程度50%,2次压缩时间间隔5 s,负重探头类型为Auto-5g,数据收集率为200 pps。

1.5.4 饲料及鱼肉营养成分含量

大口黑鲈鱼肉及其基础饲料样品常规分析方法如下:水分含量的测定按照国标GB 5009.3—2010《食品中水分的测定》中的直接干燥法,粗灰分含量的测定按照国标GB 5009.4—2016《食品中灰分的测定》中马弗炉高温灼烧法,粗蛋白质含量的测定按照国标GB 5009.5—2016《食品中蛋白质的测定》中凯氏定氮法,粗脂肪含量的测定按照国家标准GB 5009.6—2016《食品中脂肪的测定》中索氏抽提法,脂肪酸组成及含量的测定按照国家标准GB 5009.168—2016《食品中脂肪酸的测定》,氨基酸组成及含量的测定按照国家标准GB 5009.124—2016《食品中氨基酸的测定》。

1.5.5 肌肉中土腥味物质含量

参考王侯宇等[32]的方法,称取鱼糜样品2.00 g,加入2 mL纯水,均浆1 min。加入4 μg/L内标IBMP溶液,匀浆1 min。再加入5 mL乙腈,涡旋振荡1 min,静置3 min,加入1 g氯化钠,涡旋振荡1 min,加入5 g无水硫酸钠,涡旋振荡1 min,4 ℃条件下4 500 r/min离心10 min,取上清液2 mL,依次加入C18和PSA各0.1 g,涡旋混合1 min,4 ℃条件下4 500 r/min离心10 min,取上清液过膜上机测定。
色谱条件:色谱柱为HP-5MS毛细管柱;载气为氦气;不分流进样,进样量为1 μL;进样口起始温度为250 ℃;升温程序为初始温度60 ℃,持续2.5 min,然后以15 ℃/min升至150 ℃,持续5 min,最后以5 ℃/min升至250 ℃。质谱条件:离子源温度为280 ℃;电子能量为70 eV;扫描模式为选择离子检测(selected ion monitor,SIM)。

1.5.6 肠道消化酶活性

将肠道样品于4 ℃冰箱解冻后,准确称取0.1 g肠道内容物加入9 mL的匀浆介质,匀浆后制成10%的组织均浆,2 500 r/min离心10 min,取上清液,测定肠道消化酶活性。胃蛋白酶和胰蛋白酶活性均使用南京建成生物工程研究所的试剂盒测定,具体操作步骤按照试剂盒说明书进行。

1.5.7 肠道组织切片形态学

取大口黑鲈中肠,用4%的多聚甲醛固定,然后经洗涤、脱水、浸蜡、包埋、切片、展片、脱蜡、染色、封片后,在光学显微镜下对组织切片进行观察和分析。拍照时在相同的光源下,每片大口黑鲈肠道切片放大倍数分别固定为50倍和150倍,使肠道切片全部出现在同一视野下。拍好后取肠道组织中较长的5条肠道绒毛,用ZEN 3.0软件中的比例尺测量绒毛长度和绒毛宽度,同时测量肠道组织的肌层厚度(μm)。

1.5.8 前肠短链脂肪酸含量

称取约50 mg粪便,并记录粪便重量,加入250 μL纯水均质5 min,再加入10 μL 5 mol/L盐酸,均质1 min,静置5 min,再均质5 min,静置5 min,随后在4 ℃条件下12 000 r/min离心10 min。移取200 μL上清液,加入内标2-乙基丁酸(浓度为1 mmol/L),涡旋1 min,12 000 r/min离心5 min。吸取上清液过水系滤膜后,置于玻璃衬管,再放入棕色进样瓶中即可。
气相色谱法测定:采用DB-FFAP 125-3237短链脂肪酸分析柱(30 m×0.52 mm×0.50 mm,美国Agilent Technologies公司)。柱箱升温参数:初始值为100 ℃,运行0.5 min;后以8 ℃/min的升温速率升高到180 ℃,运行1.0 min,以20 ℃/min的升温速率升高到200 ℃,运行15 min。FID检测器温度为240 ℃,氢气流量、空气流量和尾吹氮气流量分别为30、300和20 mL/min;进样口温度为200 ℃,氮气总流量为6.0 mL/min;进样量为1 μL,运行时间为27.5 min。

1.5.9 DNA提取及16S rRNA基因测序

大口黑鲈后肠内容物DNA提取按照Qiagen QIAamp DNA Stool Mini Kit说明书,具体操作步骤如下:准确称取大口黑鲈粪便40 mg置于冰上的2 mL离心管中,加入0.5 mL Inhibit EX Buffer缓冲液,涡旋振荡至样本完全均质;然后离心(15 000 r/min,1 min);取300 μL上清液置于20 μL Proteinase K的离心管中,加入300 μL Buffer AL缓冲液,涡旋振荡16 s,70 ℃加热10 min,加入300 μL无水乙醇,涡旋均质;准确移取上一步中的裂解液600 μL至QIAamp离心吸附柱中,然后移至收集管中离心(15 000 r/min,1 min);离心后将吸附柱移入新的收集管中,向吸附柱内加入500 μL Buffer AW1缓冲液,离心(15 000 r/min,1 min);再将吸附柱移入新的收集管中,向吸附柱内加入500 μL Buffer AW2缓冲液,离心(15 000 r/min,3 min),吸附柱移入新的收集管中,再次离心(15 000 r/min,3 min);将吸附柱换入新的离心管中,加入80 μL Buffer ATE值吸附滤膜,25 ℃下孵育2 min,离心(15 000 r/min,1 min),存于-80 ℃待测。通过Thermo NanoDrop 2000核酸浓度检测仪和1%的琼脂糖凝胶电泳检测大口黑鲈提取的粪便DNA纯度。
文库的构建和测序方法如下:通过引物序列33F(ACTCCTACGGGAGGCAGCAG)和806R(GGACTACHVGGGTWTCTAAT)用于PCR扩增16S rRNA的V3~V4区。使用KAPA HiFi Hoststant ReadyMix PCR Kit进行PCR,琼脂糖凝胶电泳检测PCR产物,AxyPrep DNA凝胶试剂盒回收PCR产物,回收产物用Nanodrop 2000核酸浓度仪和1%的琼脂糖凝胶电泳测量纯度,使用Qubit 2.0荧光分光光度计进行定量,并将各样本文库进行等摩尔混合。使用Illumina HiSeq2500 PE 250进行测序;通过FLASH软件进行序列的拼接后得到较长的序列;利用Usearch软件去除嵌合体,进行标准聚类,相似度≥97%的序列组成1个操作分类单元(operational taxonomic unit,OTU),每1个OTU代表1个物种;利用QIIME软件挑出每个物种的代表序列,将OTU的序列和Silva128/16S数据库比对,进行OTU物种信息注释。
表1 基础饲料组成及营养水平(风干基础)

Table 1 Composition and nutrient levels of the basal diet (air-dry basis)

项目 Items 含量 Content
原料 Ingredients/(g/kg)
鱼粉 Fish meal 360.0
豆粕 Soybean meal 216.0
谷朊粉 Wheat gluten 70.0
鱼油 Fish oil 30.0
大豆油 Soybean oil 20.0
小麦粉 Wheat meal 212.0
酵母粉 Yeast meal 20.0
卵磷脂 Lecithin 25.0
矿物质预混料 Mineral premix1) 20.0
维生素预混料 Vitamin premix2) 20.0
抗氧化剂 Antioxidant 0.5
诱食剂 Attractant 3.0
防霉剂 Mold inhibitor 1.0
氯化胆碱 Choline chloride 2.5
合计 Total 1 000.0
营养水平 Nutrient levels/%3)
粗蛋白质 Crude protein 49.00
粗脂肪 Crude lipid 9.00
粗灰分 Ash 15.00
水分 Moisture 8.00

1)矿物质预混料为每千克饲料提供 Mineral premix provided the following per kg of the diet:NaF2 2 mg,KI 1 mg,CoCl2 (1%) 50 mg,CuSO4 10 mg,Fe2(SO4)3 80 mg,ZnSO4 50 mg,CuSO4 60 mg,MgSO4 1 200 mg,Ca(H2PO4)2 8 000 mg,NaCl 100 mg,沸石粉 zeolite powder 10.447 g。

2)维生素预混料为每千克饲料提供 Vitamin premix provided the following per kg of the diet:VB1 21 mg,VB2 40 mg,VB6 20 mg,VB12 0.5 mg,VK3 10 mg,肌醇 inositol 800 mg,VB5 60 mg,烟酸 niacin 200 mg,叶酸 folic acid 20 mg,VH 1.5 mg,VA 32 mg,VD3 5 mg,VE 120 mg,VC 2 000 mg,胆碱 choline 2 000 mg,乙氧基喹啉 ethoxyquin 150 mg,微晶纤维素 microcrystalline cellulose 14.52 g。

3)营养水平为实测值。Nutrient levels were measured values.

数据处理的方法如下:用QIIME和R软件比较物种组成差异和图像展示,数据以平均值±标准差表示。多组之间的差异比较采用Tukey检验或非参数性Kruskal-Wallis秩和检验进行方差和显著性分析。

1.6 数据统计与分析

试验数据采用SPSS 27.0进行单因素方差分析(one-way ANOVA),并采用Duncan氏多重比较法进行检验,确定不同组之间是否存在显著性差异(P<0.05)。采用GraphPad Prism 9.4.1作图。

2 结果与分析

2.1 混合益生菌对大口黑鲈生长性能和形体指标的影响

表2所示,各组之间生长性能和形体指标无显著差异(P>0.05)。与CON组相比,MP-0.1%和MP-1.0%组的存活率分别提高了9.6%和11.55%,增重率分别提高了1.87%和16.77%,饲料效率分别提高了6.98%和11.63%,特定生长率分别提高了0.85%和8.55%,且以上指标MP-1.0%组均高于MP-0.1%组;MP-0.1%和MP-1.0%组的肝体比和脏体比均有所升高,但MP-1.0%组却低于MP-0.1%组。
表2 混合益生菌对大口黑鲈生长性能和形体指标的影响

Table 2 Effects of mixed probiotics on growth performance and shape indexes of largemouth bass

指标
Items
组别 groups
CON MP-0.1% MP-1.0%
存活率 SR/% 88.19±9.35 96.66±6.39 98.38±2.64
增重率 WGR/% 360.37±60.44 367.10±81.37 420.81±30.81
饲料效率 FCR 0.86±0.10 0.92±0.09 0.96±0.01
特定生长率 SGR/(%/d) 1.17±0.10 1.18±0.14 1.27±0.05
肥满度 CF/(g/cm3) 3.07±0.20 3.11±0.15 2.99±0.04
肝体比 HI/% 2.01±0.15 2.16±0.57 2.03±0.25
脏体比 VI/% 7.26±1.34 8.01±1.09 7.41±1.19

同行数据肩标不同小写字母表示差异显著(P<0.05),相同或无字母表示差异不显著(P>0.05)。下表同。

In the same row, values with different small letter superscripts mean significant difference (P<0.05), while with the same or no letter superscripts mean no significant difference (P>0.05). The same as below.

2.2 混合益生菌对大口黑鲈肉品质的影响

2.2.1 肌肉纤维形态分析

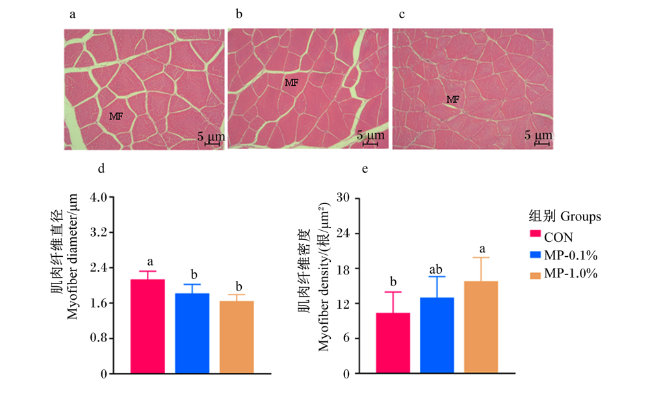
图1所示,MP-1.0%组的肌肉纤维明显比CON组紧密;与CON组相比,MP-0.1%和MP-1.0%组的肌肉纤维直径显著降低(P<0.05),MP-1.0%组的肌肉密度显著升高(P<0.05)。总体来看,肌肉纤维直径的大小随着混合益生菌的添加水平的增加而减小,肌肉纤维密度随着混合益生菌添加水平的增加而升高。
图1 混合益生菌对大口黑鲈肌肉纤维形态的影响

a~c:横切面肌肉纤维结构,放大100倍;a:CON组,b:MP-0.1%组,c:MP-1.0%组。d~e:肌肉纤维直径和肌肉纤维密度。MF:肌肉纤维。
数据柱标相同小写字母表示差异不显著(P>0.05),不同小写字母表示差异显著(P<0.05)。下图同。

Fig.1 Effects of mixed probiotics on myofiber morphology of largemouth bass

a to c: myofiber structure of cross sections, magnification is 100; a: CON group, b: MP-0.1% group, c: MP-1.0% group. d and e: myofiber diameter and myofiber density. MF: myofiber.
Value columns with the same small letter mean no significant difference (P>0.05), while with different small letters mean significant difference (P<0.05). The same as below.

2.2.2 肌肉质构特性分析

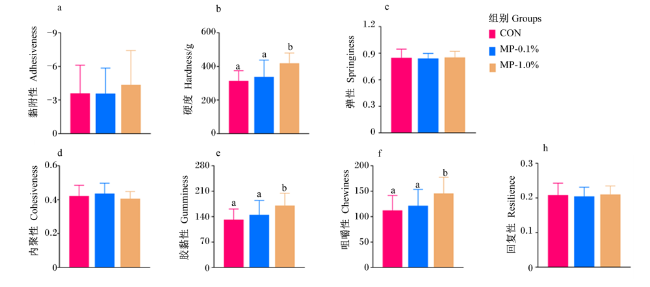
图2所示,各组之间肌肉黏附性、弹性、内聚性和回复性均无显著差异(P>0.05)。与CON组相比,MP-1.0%组的肌肉硬度、胶黏性和咀嚼性显著升高(P<0.05)。
图2 混合益生菌对大口黑鲈肌肉质构特性的影响

Fig.2 Effects of mixed probiotics on muscle texture characteristics of largemouth bass

2.2.3 肌肉营养成分分析

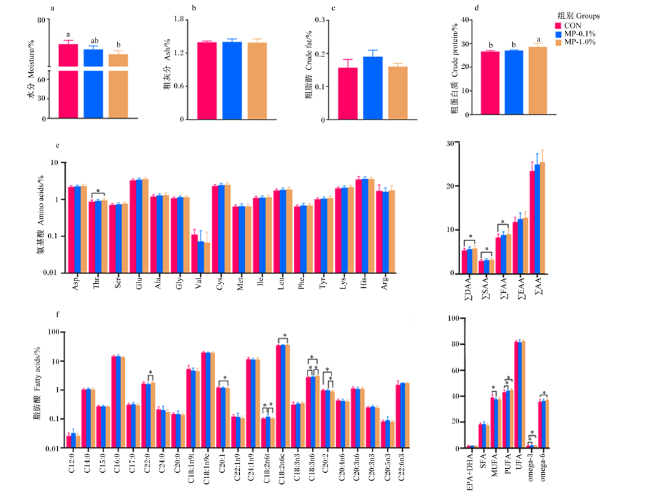
图3所示,各组之间肌肉粗灰分和粗脂肪含量均无显著差异(P>0.05)。与CON组相比,MP-1.0%组的肌肉水分含量显著降低(P<0.05),肌肉粗蛋白质、风味氨基酸(鲜味氨基酸、甜味氨基酸)、多不饱和脂肪酸、omega-3脂肪酸及omega-6脂肪酸含量显著升高(P<0.05);MP-0.1%组的肌肉多不饱和脂肪酸和omega-3脂肪酸含量显著升高(P<0.05),而肌肉单不饱和脂肪酸含量显著下降(P<0.05)。整体来看,大口黑鲈肌肉营养成分含量随着混合益生菌添加水平的增加而升高。
图3 混合益生菌对大口黑鲈肌肉营养成分含量的影响

Asp:天冬氨酸;Thr:苏氨酸;Ser:丝氨酸;Glu:谷氨酸;Ala:丙氨酸;Gly:甘氨酸;Val:缬氨酸;Cys:半胱氨酸;Met:蛋氨酸;Ile:异亮氨酸;Leu:亮氨酸;Phe:苯丙氨酸;Tyr:酪氨酸;Lys:赖氨酸;His:组氨酸;Arg:精氨酸;DAA:鲜味氨基酸(天冬氨酸+谷氨酸);SAA:甜味氨基酸(丝氨酸+甘氨酸+丙氨酸);FAA:风味氨基酸(鲜味氨基酸+甜味氨基酸);EAA:必需氨基酸;TAA:总氨基酸;SFA:饱和脂肪酸;MUFA:单不饱和脂肪酸;PUFA:多不饱和脂肪酸;UFA:不饱和脂肪酸。*表示差异显著(P<0.05)。

Fig.3 Effects of mixed probiotics on muscle nutrient contents of largemouth bass

Asp: aspartate; Thr: threonine; Ser: serine; Glu: glutamate; Ala: alanine; Gly: glycine; Val: valine; Cys: cysteine; Met: methionine; Ile: isoleucine; Leu: leucine; Phe: phenylalanine; Tyr: tyrosine; Lys: lysine; His: histidine; Arg: arginine; DAA: delicious amino acids (Asp+Glu); SAA: sweet amino acids (Ser+Gly+Ala); FAA: flavor amino acids (DAA+SAA); EAA: essential amino acids; TAA: total amino acids; SFA: saturated fatty acids; MUFA: monounsaturated fatty acids; PUFA: polyunsaturated fatty acids; UFA: unsaturated fatty acids. * mean significantly different (P<0.05).

2.2.4 肌肉中土腥味物质含量分析

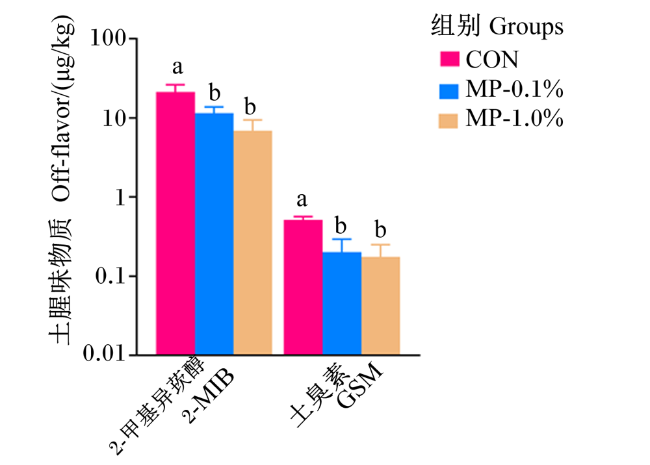
图4所示,与CON组相比,MP-0.1%和MP-1.0%组的肌肉中土臭素和2-甲基异莰醇含量均显著降低(P<0.05)。
图4 混合益生菌对大口黑鲈肌肉中土腥味物质含量的影响

Fig.4 Effects of mixed probiotics on muscle off-flavor contents of largemouth bass

2.3 混合益生菌对大口黑鲈肠道健康的影响

2.3.1 肠道消化酶活性分析
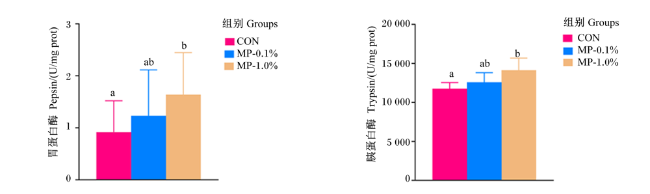
图5所示,与CON组相比,MP-1.0%组的肠道胃蛋白酶和胰蛋白酶活性均显著升高(P<0.05)。
图5 混合益生菌对大口黑鲈肠道消化酶活性的影响

Fig.5 Effects of mixed probiotics on intestinal digestive enzyme activities of largemouth bass

2.3.2 肠道组织形态分析

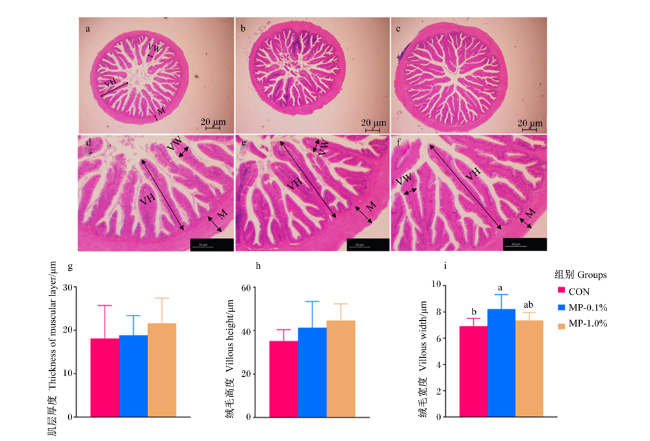
图6所示,与CON组相比,MP-0.1%组的肠道绒毛宽度显著提高(P<0.05)。各组之间肌层厚度和绒毛高度无显著差异(P>0.05)
图6 混合益生菌对大口黑鲈肠道组织形态的影响

a~f:横切面肠道组织形态;a~c为放大50倍,d~f为放大150倍,a和d为CON组,b和e为MP-0.1%组,c和f为MP-1.0%组。M:肌层厚度;VW:绒毛宽度;VH:绒毛高度。

Fig.6 Effects of mixed probiotics on intestinal morphology of largemouth bass

a to f: intestinal morphology in cross section; a to c magnification is 50, d to f magnification is 150; a and d were CON group, b and e were MP-0.1% group, c and f were MP-1.0% group. M: muscular layer thickness; VW: villous width; VH: villous height.

2.3.3 肠道短链脂肪酸含量分析

表3所示,在大口黑鲈肠道中发现4种短链脂肪酸,与CON组相比,MP-0.1%组的肠道乙酸、丙酸、丁酸、异戊酸及总酸含量均有所升高,但差异不显著(P>0.05);MP-1.0%组的肠道异戊酸和总酸含量显著升高(P<0.05),乙酸、丙酸和丁酸含量均有所升高,但差异不显著(P>0.05)。
表3 混合益生菌对大口黑鲈肠道短链脂肪酸含量的影响

Table 3 Effects of mixed probiotics on intestinal short-chain fatty acid contents of largemouth bassmmol/mg

项目
Items
组别 Groups
CON MP-0.1% MP-1.0%
乙酸 Acetic acid 18.51±3.09 18.94±1.95 19.50±3.19
丙酸 Propanoic acid 3.27±1.34 3.39±1.04 3.56±0.93
丁酸 Butyric acid 3.29±1.74 3.43±1.76 3.61±1.11
异戊酸 Isovaleric acid 4.68±2.00a 4.73±2.04a 6.36±2.01b
总酸 Total acid 29.76±2.56a 30.49±2.85ab 33.03±4.69b

2.3.4 肠道菌群分析

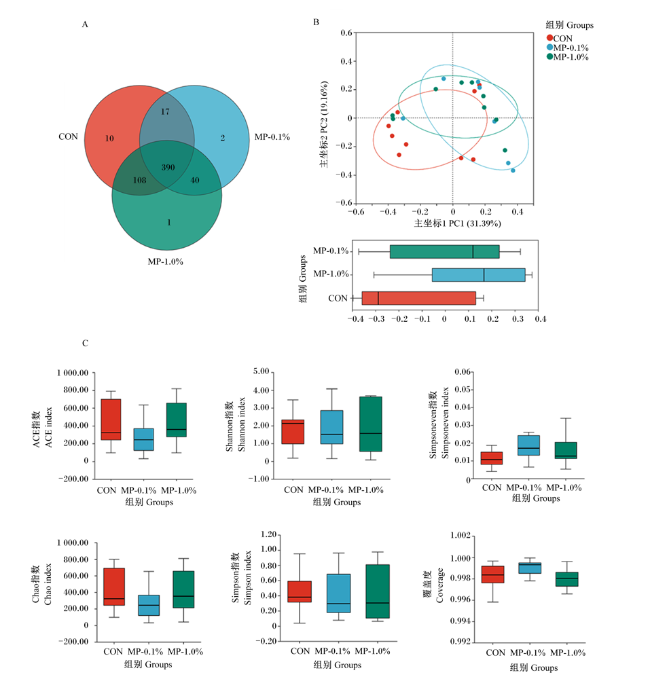
为了进一步探究混合益生菌对大口黑鲈肠道菌群的影响,本试验基于16S rRNA高通量测序技术,对大口黑鲈肠道菌群多样性进行了分析测定。共检测到568个OTU,其中3组共有390个OTU,CON、MP-0.1%和MP-1.0%组独有的OTU数量分别是10、2和1个(图7-A),说明CON组肠道菌群组成较混合益生菌组差异更大。此外,还对大口黑鲈的肠道菌群的α多样性和β多样性进行分析,α多样性代表菌群的丰度差异,β多样性代表菌群的组成差异。主坐标分析(PCoA)结果显示,CON组与MP-0.1%和MP-1.0%组聚类明显,且几乎没有交叉,而MP-0.1%和MP-1.0%组交叉严重,说明混合益生菌显著影响了大口黑鲈肠道微生物的组成(图7-B)。混合益生菌对大口黑鲈肠道菌群的α多样性无显著影响(P>0.05)(图7-C)。
图7 混合益生菌对大口黑鲈肠道菌群多样性的影响

A:韦恩图;B:β-多样性;C:α-多样性。

Fig.7 Effects of mixed probiotics on gut microbiota diversity of largemouth bass

A: Venne chart; B: β-diversity; C: α-diversity.

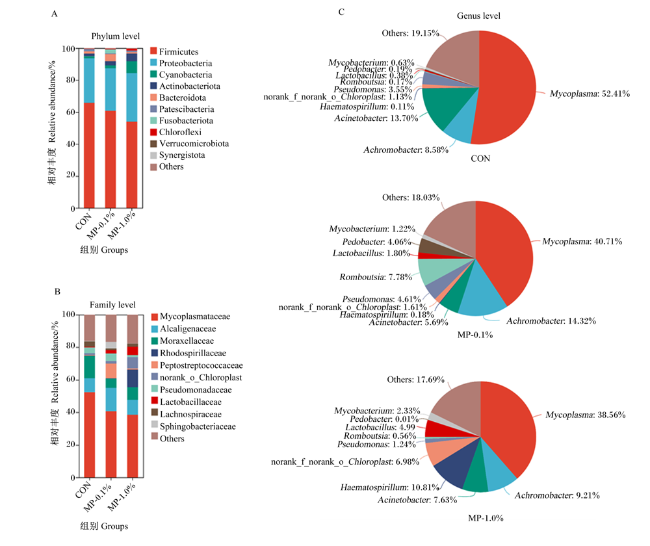
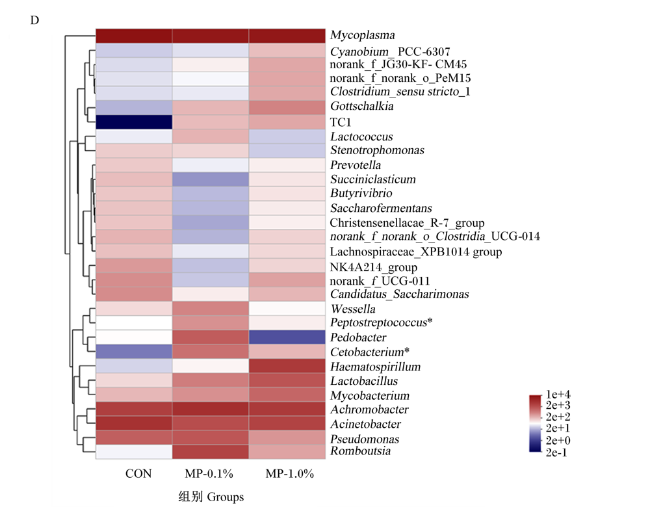
鱼类肠道中的优势共生菌群对鱼类消化吸收、营养代谢和免疫调节起着至关重要的作用。通过对大口黑鲈进行16S rRNA高通量测序,对大口黑鲈肠道菌群的结构及功能进行了分析测定。分类学结果表明,在门水平上,大口黑鲈的肠道菌群主要由厚壁菌门(Firmicutes)和变形菌门(Proteobacteria)组成,这2种菌门相对丰度总计占比超过了80%,是大口黑鲈的优势菌群,并且肠道中厚壁菌门相对丰度随着混合益生菌添加剂水平的增加而下降,蓝藻门(Cyanobacteria)、放线菌门(Actinobacteriota)和绿弯菌门(Chloroflexi)相对丰度随着混合益生菌添加水平的增加而增加,具有剂量依赖效应(图8-A)。在科水平上,菌群组成进一步分化,相对丰度最高的是支原体科(Mycoplasmataceae),该科属于厚壁菌门,并且肠道中支原体科相对丰度随着混合益生菌添加水平的增加而下降,红螺菌科(Rhodospirillaceae)、叶绿体(norank_o_Chloroplast)和乳杆菌科(Lactobacillaceae)相对丰度随着混合益生菌添加水平的增加而增加,具有剂量依赖性应(图8-B)。在属水平上,肠道中支原体菌属(Mycoplasma)的占比随着混合益生菌添加水平的增加而下降,Haematospirillum、norank_f_norank_o_Chloroplast、乳酸杆菌属(Lactobacillus)和分枝杆菌属(Mycobacterium)的占比随着混合益生菌添加水平的增加而增加,具有剂量依赖性效应(图8-C)。此外,鲸杆菌属(Cetobacterium)和消化链球菌属(Peptostreptococcus)在3组之间有显著差异(P<0.05)(图9)。
图8 混合益生菌对大口黑鲈肠道菌群组成的影响(相对丰度前10)

Phylum level:门水平;Family level:科水平;Genus level:属水平。Firmicutes:厚壁菌门;Proteobacteria:变形菌门;Cyanobacteria:蓝藻门;Actinobacteriota:放线菌门;Bacteroidota:拟杆菌门;Patescibacteria:候选菌门;Fusobacteriota:梭杆菌门;Chloroflexi:绿弯菌门;Verrucomicrobiota:疣微菌门;Synergistota:互养菌门。Mycoplasmataceae:支原体科;Alcaligenaceae:产碱菌科;Moraxellaceae:莫拉氏菌科;Rhodospirillaceae:红螺菌科;Peptostreptococcaceae:消化链球菌科;norank_o_Chloroplast:叶绿体;Pseudomonadaceae:假单胞菌科;Lactobacillaceae:乳杆菌科;Lachnospiraceae:毛螺菌科;Sphingobacteriaceae:鞘氨醇杆菌科。Mycoplasma:支原体菌属;Pedobacter:土地杆菌属;Lactobacillus:乳酸杆菌属;Mycobacterium:分支杆菌属;Achromobacter:无色杆菌属;Acinetobacter:不动杆菌属;Pseudomonas:假单胞菌属;Romboutsia:罗姆布茨菌属。
A:肠道菌群门水平组成柱形图;B:肠道菌群科水平组成柱形图;C:肠道菌群属水平组成饼图。

Fig.8 Effects of mixed probiotics on gut microbiota composition of largemouth bass (top 10 relative abundance)

A: histogram of the horizontal composition of the intestinal flora phylum; B: histogram of the horizontal composition of the intestinal flora family; C: pie chart of genus-level composition of the intestinal flora.

图9 混合益生菌对大口黑鲈肠道菌群属水平组成的影响(相对丰度前30)

Cyanobium:蓝藻菌属;Lactococcus:乳球菌属;Stenotrophomonas:寡养单胞菌属;Prevotella:普氏菌属;Succiniclasticum:琥珀酸弧菌属;Butyrivibrio:丁酸弧菌属;Saccharofermentans:产乙酸糖发酵菌属;Christensenellaceae R-7_group:克里斯滕森菌科R-7组;norank_f_norank_o_Clostridia_UCG-014:梭状芽孢杆菌属UCG-014;Lachnospiraceae_XPB1014_group:毛螺菌科XPB1014组;Weissella:魏斯氏菌属;Peptostreptococcus:消化链球菌属;Cetobacterium:鲸杆菌属。
*表示差异显著(P<0.05)。

Fig.9 Effects of mixed probiotics on genus level composition of gut microbiota of largemouth bass (top 30 relative abundance)

* mean significant difference (P<0.05).

3 讨论

3.1 混合益生菌对大口黑鲈生长性能和形体指标的影响

鱼类的生长性能和形体指标不仅是评价其生长和营养状况的初级指标,还是评价其商品经济价值的重要指标之一[33]。生长性能主要包含存活率、增重率、饲料效率和特定生长率等指标,形体指标主要包含肥满度、肝体比和脏体比等指标。在本试验中,混合益生菌对大口黑鲈的生长性能和形体指标虽然无显著影响,但提高了大口黑鲈的存活率、增重率、饲料效率和特定生长率。分析其原因,首先饲料中补充混合益生菌能够提高肠道消化酶活性,增强对营养物质的利用,从而促进鱼体的生长[34];其次饲料中补充混合益生菌能够增加宿主肠道短链脂肪酸含量,短链脂肪酸不仅能够为肠道上皮细胞提供能量,保护肠道黏膜屏障,刺激肠道消化酶的产生,提高机体对营养物质的吸收利用,还能通过调节肠道微生物组成,促进机体有益菌的生长,从而增强鱼体免疫力,提高存活率[35]。Tao等[36]试验也发现,在大口黑鲈饲料中添加益生菌可以提高增重率和特定生长率,并在嗜水气单胞菌(Aeromonas hydrophila)感染测试中显著提升累计存活率。邓希海等[37]研究发现,以枯草芽孢杆菌(Bacillus subtilis)为主的益生菌制剂能够显著提高大口黑鲈的增重率、特定生长率、抗氧化能力和免疫力。此外,研究者们在草鱼(Ctenopharyngodon idellus)[38]、鲤鱼(Cyprinus carpio)[22]、西伯利亚鲟(Acipenser baerii)[12]、尼罗罗非鱼(Oreochromis niloticus)[39]等其他水产动物中也得出相似的结果。这说明饲料中适量添加混合益生菌能够提高大口黑鲈的生长性能,并不影响其形体指标。

3.2 混合益生菌对大口黑鲈肌肉质构特性和纤维结构的影响

鱼肉的质构特性与肉质的口感密切相关,通常认为,大口黑鲈肌肉的质构硬度较大,弹性较强时,口感更好[40-41]。鱼肉的质构特性还与鱼体营养密切相关,鱼肉质构硬度与鱼体水分含量呈负相关,水分含量越高,肉质越细嫩[42]。在本试验中,与CON组相比,MP-1.0%组的硬度、黏附性和咀嚼性显著升高。原因其分析,一方面可能是由于混合益生菌的添加提高了大口黑鲈的饲料利用率,促进了对营养物质的吸收,增加了肌肉中粗蛋白质含量,肌肉中粗蛋白质含量升高有助于肌原纤维蛋白的生长,而肌原纤维蛋白与质构弹性呈正相关[43];另一方面可能是由于肌肉中水分含量的降低,有研究表明鱼肉的质构硬度与水分含量呈负相关[42]
有研究表明,肌肉纤维直径与鱼肉的硬度、弹性和咀嚼性呈负相关[44],也就是说肌肉纤维直径越短、纤维密度越高,硬度和弹性就越强[45]。本试验结果也验证了这一观点。本试验中,与CON组相比,MP-0.1%和MP-1.0%组的肌肉纤维直径显著下降,MP-1.0%组的肌肉纤维密度显著增加。这也与国内外其他学者报道的结果保持一致。Wang等[46]在饲料中添加干酪乳杆菌K17(Lactobacillus casei K17),显著提高了大口黑鲈肌肉纤维密度、硬度、咀嚼性和胶黏性。夏雨等[47]在饲料中添加植物乳杆菌,提高了凡纳滨对虾(Litopenaeus vannamei)肌肉弹性和咀嚼性。这说明饲料中添加适量混合益生菌可以提升大口黑鲈肉质口感。

3.3 混合益生菌对大口黑鲈肌肉营养价值的影响

营养价值是评价鱼肉品质的重要指标,水产动物不仅是优质蛋白质的来源,也含有丰富的不饱和油脂资源[48]。本试验中,与CON组相比,MP-1.0%组的肌肉水分含量显著降低,肌肉粗蛋白质含量显著提高,而肌肉粗脂肪含量并无显著差异。分析其原因,混合益生菌的添加可以通过提高鱼体消化酶活性、肠道肌层厚度、绒毛长度和绒毛宽度等,从而增加对营养物质的吸收[38,49-50]。此外,在益生菌饲喂下的鲫鱼(Carassius auratus)[51]、尼罗罗非鱼[25]、真鲷(Pagrus major)[26]、红罗非鱼(Oreochromis spp)等水产动物肌肉粗蛋白质含量也显著提升,与本试验结果一致。这说明饲料中添加适量混合益生菌可以提升大口黑鲈肌肉营养价值。
蛋白质的基本组成单位氨基酸不仅是反映蛋白质质量的重要指标,也是反映风味的重要指标。本研究结果显示,饲料中添加混合益生菌提高了大口黑鲈肌肉中必需氨基酸含量,其中苏氨酸含量显著升高,苏氨酸参与蛋白质的合成,促进生长,还能够增强机体免疫力[52]。对于风味氨基酸,与CON组相比,MP-1.0%组的肌肉风味氨基酸含量显著增加,包括鲜味氨基酸和甜味氨基酸。分析其原因:饲料中添加混合益生菌可以提高大口黑鲈肠道中有益菌的生长繁殖,提高肠道中短链脂肪酸含量,促进肠道绒毛的生长及提高肠道消化酶活性,从而增加对营养物质的吸收利用,进而提高了机体总氨基酸和风味氨基酸含量。王劲松等[53]研究发现,饲喂干酪乳杆菌K17显著提高了加州鲈肌肉中甜味氨基酸和鲜味氨基酸含量。此外,饲料中添加益生菌的淇河鲫鱼和云斑尖塘鳢等水产动物肌肉中风味氨基酸和必需氨基酸含量均显著升高[54-55]。因此,饲料中添加适量的混合益生菌不仅可以提高大口黑鲈肌肉中有益人体健康的氨基酸含量,还能有效提高鱼肉风味。
脂肪酸分为饱和脂肪酸和不饱和脂肪酸,饱和脂肪酸存在诱发多种疾病的潜在危害[56-57],而不饱和脂肪酸有利于缓解一些代谢综合征[58],特别是omega-3脂肪酸对人体的免疫、细胞的组成和发育、血液的健康及抗癌等方面发挥着积极的作用[59-60]。本研究中,与CON组相比,饲料中添加混合益生菌后大口黑鲈肌肉中多不饱和脂肪酸和omega-3脂肪酸含量显著提高,且MP-1.0%组的肌肉中omega-6脂肪酸含量显著升高,但MP-0.1%组的肌肉中单不饱和脂肪酸含量显著降低。分析其原因:首先混合益生菌通过促进宿主消化酶的表达和肠道绒毛的生长,改善胃肠道的消化功能,提高对营养物质的吸收;其次可能是由于部分益生菌自身代谢产生不饱和脂肪酸,从而增加肌肉中不饱和脂肪酸含量,并已有一些肠道微生物被认为可能是多不饱和脂肪酸的生产菌株[47,61]。夏雨等[47]在饲料中添加植物乳杆菌,提高了凡纳滨对虾肌肉中不饱和脂肪酸含量,降低了饱和脂肪酸含量。Hossain等[62]给似野结鱼(Tor tambroides)饲喂益生菌后,鱼体的单不饱和脂肪酸及omega-6脂肪酸含量显著升高,与本研究结果相似。饲料中添加混合益生菌后,虽然大口黑鲈肌肉中单不饱和脂肪酸含量有所下降,但对人体有利的其他脂肪酸含量显著升高。

3.4 混合益生菌对大口黑鲈肌肉中土腥味物质含量的影响

水产品中的土腥味物质主要来自于养殖水体中放线菌、霉菌和蓝藻产生的次级代谢产物土臭素和2-甲基异莰醇[63-64],这些土腥味物质随之被鱼体吸收,并在鱼体内蓄积,对水产品风味造成严重的不良影响。因此,降低鱼肉中土腥味物质含量,提高鱼肉品质是大口黑鲈发展面临的主要问题[65]。本研究中,饲料中添加混合益生菌后大口黑鲈肌肉中土腥味物质含量显著降低。分析其原因,可能是由于饲料中没有定植和消化的益生菌随粪便排入水体,通过降解有机废物,稳定水体环境,减少鱼体不良气味的蓄积[66]。已有研究表明,微生态制剂能够降低水体中氨氮和亚硝酸盐含量[67]。这说明在饲料中添加适量混合益生菌可降低大口黑鲈生长过程中不良风味的蓄积,提升鱼肉品质,但其具体的机理还有待研究。

3.5 混合益生菌对大口黑鲈肠道消化酶活性的影响

消化酶主要是由消化系统和消化腺产生的,鱼类肠道中消化酶活性是反映其消化吸收能力的重要指标,也是鱼类正常生长的重要保障[68]。其中,大口黑鲈肠道中的前肠消化酶活性最高,为消化酶活性测定的最适肠段。益生菌可以通过调节宿主肠道微生态及其代谢,提高消化酶活性[69]。本试验中,饲料中添加混合益生菌提高了大口黑鲈肠道中胃蛋白酶和胰蛋白酶活性。分析其原因,首先部分益生菌自身代谢会产生一些酶类使得鱼体内消化酶活性提高[34,70];其次在饲喂混合益生菌期间,部分益生菌代谢产生短链脂肪酸,从而对鱼体肠道产生刺激,促使鱼体消化酶的分泌[71]。李岩[69]在饲料中添加植物乳杆菌,显著提高了大口黑鲈的肠道消化酶活性。此外,研究者们发现在乌鳢(Channa argus)、石斑鱼(Epinephelus coioides)和鲤鱼等其他水产动物中也得出相似结论[30,72-73]。这说明饲料中添加适量混合益生菌可以增强大口黑鲈肠道消化酶活性,提高对营养物质的消化吸收能力。

3.6 混合益生菌对大口黑鲈肠道组织结构的影响

肠道是鱼类消化吸收的主要器官,因此肠道的发育直接影响饲料中营养物质的吸收利用,从而影响鱼类的生长和健康[74]。肠道绒毛高度和肌层厚度与肠道营养物质的吸收成正比[69],许多研究者通过鱼体肠道结构来评价其肠道生长发育的健康程度。本研究发现,饲料中添加混合益生菌可以提高大口黑鲈肠道的绒毛高度和绒毛宽度,增加绒毛面积,从而提高对饲料中营养物质的吸收。其分析原因,大口黑鲈肠道组织结构的改变可能与微生物代谢产生的表面活性素和酸类物质有关,如丁酸、乳酸等,这些物质能够促进肠道细胞的增殖和肠道的蠕动[75]。张冬梅等[7]在饲料中添加枯草芽孢杆菌,发现大口黑鲈幼鱼肠道绒毛高度、绒毛数量和肌层厚度均显著提高。Wang等[50]研究发现,在饲料中添加乳杆菌能够提高大口黑鲈绒毛面积。研究还发现,在益生菌饲喂下的大西洋鲑(Salmo salar)、异育银鲫(Carassius auratus gibelio)和大菱鲆(Scophthalmus maximus)等水产动物中也显示出类似结果[76-78]。这说明饲料中添加适量混合益生菌可以促进大口黑鲈肠道生长,提高对营养物质的消化吸收能力。

3.7 混合益生菌对大口黑鲈肠道短链脂肪酸含量的影响

短链脂肪酸也称为挥发性脂肪酸,主要来自肠道中微生物的代谢和发酵[79]。短链脂肪酸是肠道上皮细胞的主要能量来源,维持和保护肠道黏膜屏障和调节新陈代谢的功能,抑制病原微生物的生长繁殖和促炎因子的生成[80-81],大多数鱼类肠道中不同肠区的短链脂肪酸比例接近。常见的短链脂肪酸有甲酸、乙酸、丙酸、丁酸等,各类短链脂肪酸及其代谢产物对于提高水产动物的生长性能、营养代谢也在多项研究中得到验证[82],如在高贝尔湖红点鲑(Salvelinus alpinus)饲料中添加乙酸盐,其增重率显著提高[83];在尼罗罗非鱼饲料中添加丙酸盐,其饲料利用率和粗蛋白质含量显著提高[84];在海鲷(Dicentrarchus labrax)饲料中添加丁酸,其增重率、核苷酸衍生物及几种常见的氨基酸利用率有所提高[85]。本试验中,饲料中添加混合益生菌可以提高大口黑鲈肠道中乙酸、丙酸、丁酸、异戊酸及总酸含量。分析其原因,混合益生菌刺激了大口黑鲈肠道菌群代谢,产生短链脂肪酸,提高了肠道中短链脂肪酸含量。此外,短链脂肪酸含量的升高与肠道消化酶活性的提高和肠道绒毛生长呈正相关,这也验证了我们前面的推测。Meng等[86]在鲤鱼饲料中添加丁酸梭菌(Clostridium butyricum),发现肠道中正丁酸含量显著升高。袁海林等[35]在凡纳滨对虾饲料中添加丁酸梭菌芽孢,发现其肠道中乙酸、丙酸、丁酸、戊酸和总酸含量均显著提高。这说明饲料中添加适量混合益生菌可以提高大口黑鲈肠道短链脂肪酸含量,促进肠道及肠道益生菌的生长代谢,改善肠道和鱼体健康状态,增加对营养物质的利用率,促进鱼体生长。

3.8 混合益生菌对大口黑鲈肠道菌群的影响

鱼类肠道菌群与其生长和健康息息相关,在鱼体营养成分、生理代谢和免疫过程中发挥着重要的作用,而益生菌在鱼类肠道健康调节中具有一定的作用[87],通常益生菌在鱼类肠道的后肠中含量最高,也是最适的肠道微生物测定肠段。在本研究中,各组之间的α多样性并无显著差异,但相较于CON组,MP-0.1%和MP-1.0%组的肠道菌群多样性(Shannon和Simpson指数)略有下降,其中MP-1.0%组的丰富度(ACE和Chao指数)也略有下降。这可能是由于复合益生菌进入鱼体后,与鱼体中的有害菌产生互斥反应。此外,韦恩图中MP-0.1%和MP-1.0%组独有的OTU数目也低于CON组独有的OUT数。樊英等[88]研究也发现,饲料中添加丁酸梭菌和凝结芽孢杆菌后,虹鳟(Oncorhynchus mykiss)的肠道菌群α多样性下降;王颖[89]在黄鳝的饲料中添加复合益生菌后,肠道菌群α多样性下降。这说明饲料中添加混合益生菌能够改善大口黑鲈肠道菌群结构。并且在β多样性中还发现,CON组与MP-0.1%和MP-1.0%组之间分区明显,也说明了混合益生菌的添加改变了大口黑鲈肠道菌群结构。
本试验中,大口黑鲈肠道菌群门水平的优势菌群主要为厚壁菌门和变形菌门,也是大口黑鲈的常见菌群[74,90]。其中,厚壁菌门相对丰度随着混合益生菌的添加呈现下降,这主要是由于支原体菌科中的支原体菌属相对丰度的下调,支原体是水生动物中的致病菌,破坏宿主免疫系统,诱导其他致病菌的产生和发展[91];厚壁菌门中的乳杆菌科相对丰度随着混合益生菌添加水平的增加而升高,主要是由于乳酸杆菌属相对丰度的升高,乳酸杆菌能够降低炎症反应,维持宿主免疫功能,保护肠道屏障功能及宿主健康[92];变形菌门下的红螺菌科相对丰度随着混合益生菌添加水平的增加而升高,主要是由于Haematospirillum相对丰度的升高,Haematospirillum是一种革兰氏阴性环境微生物,现已被证明是人类病原体,但目前并未见其对于水生动物影响的研究[93]。这说明饲料中添加混合益生菌能够改善大口黑鲈肠道微生态,并具有剂量依赖效应。此外,本试验中的肠道鲸杆菌属和消化链球菌属的相对丰度上调。鲸杆菌属是淡水鱼肠道中常见的优势厌氧菌,通过调节能量代谢、免疫力和肠道健康,维持鱼体健康[92]。鲸杆菌属能够产生丁酸和维生素B12,为鱼体提供营养物质,调节肠道健康[94]。消化链球菌能够参与氨基酸的发酵,促进肠道对于氨基酸的吸收,被认为是快速生长鱼类的指示菌之一[95]。这说明饲料中添加混合益生菌能够调节大口黑鲈肠道菌群结构,改善肠道健康状况,提高鱼体免疫力及对营养物质的吸收能力。

4 结论

① 饲料中添加混合益生菌对大口黑鲈的生长性能和形体指标无显著影响。
② 饲料中添加混合益生菌能够提高大口黑鲈肌肉硬度、胶黏性和咀嚼性,增加肌肉中粗蛋白质、必需氨基酸、风味氨基酸和对人体健康有益的脂肪酸含量,降低肌肉中土腥味物质含量,提高肉品质。
③ 饲料中添加混合益生菌能够提高大口黑鲈肠道消化酶活性和短链脂肪酸含量,改善肠道形态,调节肠道微生态环境,改善肠道功能和健康状况。
④ 本试验条件下,大口黑鲈饲料中混合益生菌的适宜添加水平为1.0%。
[1]
BROWN T G, RUNCIMAN B, POLLARD S, et al. Biological synopsis of largemouth bass (Micropterus salmoides): No. 2884[R]. Nanaimo: Fisheries and Oceans Canada, 2009:1-26.

[2]
农业农村部渔业渔政管理局. 全国水产技术推广总站,中国水产学会.中国渔业统计年鉴-2022[M]. 北京: 中国农业出版社, 2022.

Fisheries and Fisheries Administration Bureau of the Ministry of Agriculture and Rural Affairs, National Fisheries Technology Extension Center,China Society of Fisheries.China fishery statistical yearbook 2022[M]. Beijing: China Agriculture Press, 2022. (in Chinese)

[3]
黄太寿, 白俊杰, 李胜杰, 等. 我国加州鲈养殖现状和绿色发展问题探讨[J]. 中国水产, 2017(12):44-47.

HUANG T S, BAI J J, LI S J, et al. Discussion on the current situation and green development of California bass farming in China[J]. China Fisheries, 2017(12):44-47. (in Chinese)

[4]
张利民, 王际英, 王世信, 等. 抗生素在水产养殖上的安全性与应用问题[J]. 齐鲁渔业, 2007, 24(11):1-4.

ZHANG L M, WANG J Y, WANG S X, et al. Safety and application issues of antibiotics in aquaculture[J]. Shandong Fisheries, 2007, 24(11):1-4. (in Chinese)

[5]
XIONG W G, SUN Y X, ZHANG T, et al. Antibiotics,antibiotic resistance genes,and bacterial community composition in fresh water aquaculture environment in China[J]. Microbial Ecology, 2015, 70(2):425-432.

[6]
NAYAK S K. Multifaceted applications of probiotic Bacillus species in aquaculture with special reference to Bacillus subtilis[J]. Reviews in Aquaculture, 2021, 13(2):862-906.

[7]
张冬梅, 颜浩骁, 罗茂林, 等. 饲料中添加枯草芽孢杆菌对大口黑鲈幼鱼生长、肠道组织结构、抗氧化能力、免疫能力和肠炎的影响[J]. 动物营养学报, 2022, 34(1):575-588.

DOI

ZHANG D M, YAN H X, LUO M L, et al. Effects of dietary Bacillus subtilis on growth,intestinal tissue structure,antioxidant capacity,immunity and enteritis of juvenile largemouth bass (Micropterus salmoides)[J]. Chinese Journal of Animal Nutrition, 2022, 34(1):575-588. (in Chinese)

[8]
李明. 混合益生菌对刺参生长、免疫、消化和肠道菌群的影响[D]. 硕士学位论文. 大连: 大连海洋大学, 2014.

LI M. Effects of probiotics on growth,immunity,digestive enzymes and intestinal microbiota in juvenile sea cucumber Apostichopus japonicus[D]. Master's Thesis. Dalian: Dalian Ocean University, 2014. (in Chinese)

[9]
CHEN X L, YI H D, LIU S, et al. Probiotics improve eating disorders in Mandarin fish (Siniperca chuatsi) induced by a pellet feed diet via stimulating immunity and regulating gut microbiota[J]. Microorganisms, 2021, 9(6):1288.

[10]
AMOAH K, HUANG Q C, TAN B P, et al. Dietary supplementation of probiotic Bacillus coagulans ATCC 7050,improves the growth performance,intestinal morphology,microflora,immune response,and disease confrontation of Pacific white shrimp,Litopenaeus vannamei[J]. Fish & Shellfish Immunology, 2019, 87:796-808.

[11]
CEBECI A, GÜRAKAN C. Properties of potential probiotic Lactobacillus plantarum strains[J]. Food Microbiology, 2003, 20(5):511-518.

[12]
POURGHOLAM M A, KHARA H, SAFARI R, et al. Dietary administration of Lactobacillus plantarum enhanced growth performance and innate immune response of Siberian sturgeon,Acipenser baerii[J]. Probiotics and Antimicrobial Proteins, 2016, 8(1):1-7.

[13]
PICCOLO G, BOVERA F, LOMBARDI P, et al. Effect of Lactobacillus plantarum on growth performance and hematological traits of European sea bass (Dicentrarchus labrax)[J]. Aquaculture International, 2015, 23(4):1025-1032.

[14]
KAZUŃ B, MAŁACZEWSKA J, KAZUŃ K, et al. Immune-enhancing activity of potential probiotic strains of Lactobacillus plantarum in the common carp (Cyprinus carpio) fingerling[J]. Journal of Veterinary Research, 2018, 62(4):485-492.

[15]
SHERIF A H, GOUDA M Y, AL-SOKARY E T, et al. Lactobacillus plantarum enhances immunity of Nile tilapia Oreochromis niloticus challenged with Edwardsiella tarda[J]. Aquaculture Research, 2021, 52(3):1001-1012.

[16]
POURGHOLAM M A, KHARA H, SAFARI R, et al. Influence of Lactobacillus plantarum inclusion in the diet of Siberian sturgeon (Acipenser baerii) on performance and hematological parameters[J]. Turkish Journal of Fisheries and Aquatic Sciences, 2017, 17(1):1-5.

[17]
SUDHA M R, CHAUHAN P, DIXIT K, et al. Molecular typing and probiotic attributes of a new strain of Bacillus coagulans-unique IS-2:a potential biotherapeutic agent[J]. Genetic Engineering and Biotechnology Journal, 2010, 2010:1-20.

[18]
FAN Y, WANG X L, WANG Y H, et al. Potential effects of dietary probiotics with Chinese herb polysaccharides on the growth performance,immunity,disease resistance,and intestinal microbiota of rainbow trout (Oncorhynchus mykiss)[J]. Journal of the World Aquaculture Society, 2021, 52(6):1194-1208.

[19]
FATH EL-BAB A F, MAJRASHI K A, SHEIKH H M, et al. Dietary supplementation of Nile tilapia (Oreochromis niloticus) with β-glucan and/or Bacillus coagulans:synergistic impacts on performance,immune responses,redox status and expression of some related genes[J]. Frontiers in Veterinary Science, 2022, 9:1011715.

[20]
XU Y J, WANG Y B, LIN J D. Use of Bacillus coagulans as a dietary probiotic for the common carp,Cyprinus carpio[J]. Journal of the World Aquaculture Society, 2014, 45(4):403-411.

[21]
GUO G X, LI K X, ZHU Q H, et al. Improvements of immune genes and intestinal microbiota composition of turbot (Scophthalmus maximus) with dietary oregano oil and probiotics[J]. Aquaculture, 2022, 547:737442.

[22]
GUPTA A, GUPTA P, DHAWAN A. Dietary supplementation of probiotics affects growth,immune response and disease resistance of Cyprinus carpio fry[J]. Fish & Shellfish Immunology, 2014, 41(2):113-119.

[23]
HOU Y F, ZHENG S P, ZOU F, et al. Lactobacillus rhamnosus 76 alleviates airway inflammation in ovalbumin-allergic mice and improves mucus secretion by down-regulating STAT6/SPDEF pathway[J]. Immunobiology, 2023, 228(5):152712.

[24]
PIRARAT N, PINPIMAI K, ENDO M, et al. Modulation of intestinal morphology and immunity in Nile tilapia (Oreochromis niloticus) by Lactobacillus rhamnosus GG[J]. Research in Veterinary Science, 2011, 91(3):e92-e97.

[25]
NOSHAIR I, KANWAL Z, JABEEN G, et al. Assessment of dietary supplementation of Lactobacillus rhamnosus probiotic on growth performance and disease resistance in Oreochromis niloticus[J]. Microorganisms, 2023, 11(6):1423.

[26]
DAWOOD M A O, KOSHIO S, ISHIKAWA M, et al. Effects of dietary supplementation of Lactobacillus rhamnosus or/and Lactococcus lactis on the growth,gut microbiota and immune responses of Red Sea bream,Pagrus major[J]. Fish & Shellfish Immunology, 2016, 49:275-285.

[27]
GONÇALVES A T, MAITA M, FUTAMI K, et al. Effects of a probiotic bacterial Lactobacillus rhamnosus dietary supplement on the crowding stress response of juvenile Nile tilapia Oreochromis niloticus[J]. Fisheries Science, 2011, 77(4):633-642.

[28]
DAWOOD M A O, KOSHIO S, ISHIKAWA M, et al. Physiological response,blood chemistry profile and mucus secretion of red sea bream (Pagrus major) fed diets supplemented with Lactobacillus rhamnosus under low salinity stress[J]. Fish Physiology and Biochemistry, 2017, 43(1):179-192.

[29]
CHOI Y M, KIM B C. Muscle fiber characteristics,myofibrillar protein isoforms,and meat quality[J]. Livestock Science, 2009, 122(2/3):105-118.

[30]
李利, 李泽健. 饲粮中添加乳酸菌对鲤鱼生长性能、鱼体组成及肠道酶活性的影响[J]. 中国饲料, 2021(13):80-83.

LI L, LI Z J. Effects of dietary Lactobacillus supplementation on growth performance,body composition and intestinal enzyme activity of common carp[J]. China Feed, 2021(13):80-83. (in Chinese)

[31]
李温蓉, 安玥琦, 陶玲, 等. 传统养殖与组合湿地-池塘循环水养殖黄颡鱼的品质比较[J]. 现代食品科技, 2023, 39(5):14-24.

LI W R, AN Y Q, TAO L, et al. Comparison of the quality of Pelteobagrus fulvidraco cultured conventionally and by the wetland-recirculating water pond combination[J]. Modern Food Science & Technology, 2023, 39(5):14-24. (in Chinese)

[32]
王侯宇, 谢晴, 张敬波, 等. 基于分散固相萃取技术的鱼体中土腥味物质的快速检测方法[J]. 食品研究与开发, 2023, 44(9):171-177.

WANG H Y, XIE Q, ZHANG J B, et al. A rapid detection method for off-flavor compounds in fish based on dispersed solid phase extraction technology[J]. Food Research and Development, 2023, 44(9):171-177. (in Chinese)

[33]
ZHANG A J, LUO W, WANG J, et al. Length-to-weight and length-to-length relations of 15 freshwater fish species (Actinopterygii:Cypriniformes) from the Oujiang River,China[J]. Acta Ichthyologica et Piscatoria, 2022, 52(1):91-93.

[34]
XU B H, WANG Y B, LI J R, et al. Effect of prebiotic xylooligosaccharides on growth performances and digestive enzyme activities of allogynogenetic crucian carp (Carassius auratus gibelio)[J]. Fish Physiology and Biochemistry, 2009, 35(3):351-357.

DOI PMID

[35]
袁海林, 李向策, 孙秋璇, 等. 丁酸梭菌芽孢对凡纳滨对虾生长性能、血清生化指标、肠道菌群及短链脂肪酸含量的影响[J]. 华南农业大学学报, 2023, 44(2):212-220.

YUAN H L, LI X C, SUN Q X, et al. Effects of Clostridium butyricum spores on growth performance,biochemical parameters in serum,intestinal flora and short-chain fatty acid content of Paneaus vannamei[J]. Journal of South China Agricultural University, 2023, 44(4):212-220. (in Chinese)

[36]
TAO J J, WANG S L, QIU H J, et al. Modulation of growth performance,antioxidant capacity,non-specific immunity and disease resistance in largemouth bass (Micropterus salmoides) upon compound probiotic cultures inclusion[J]. Fish & Shellfish Immunology, 2022, 127:804-812.

[37]
邓希海, 黄进, 刘哲. 微生态制剂对鲈鱼生长性能、血清生化指标、抗氧化能力和免疫力的影响[J]. 中国饲料, 2022(12):62-65.

DENG X H, HUANG J, LIU Z. Effects of microecological agents on growth performance,biochemical indexes,antioxidant capacity and immunity of perch[J]. China Feed, 2022(12):62-65. (in Chinese)

[38]
王颖, 宋明, 张锦华, 等. 微生态制剂对草鱼生产性能和肠道菌群的影响[J]. 水产科学, 2020, 39(1):12-21.

WANG Y, SONG M, ZHANG J H, et al. Effects of probiotics level on growth performance and intestinal flora in grass carp Ctenopharyngodon idellus[J]. Fisheries Science, 2020, 39(1):12-21. (in Chinese)

[39]
TABASSUM T, SOFI UDDIN MAHAMUD A G M, ACHARJEE T K, et al. Probiotic supplementations improve growth,water quality,hematology,gut microbiota and intestinal morphology of Nile tilapia[J]. Aquaculture Reports, 2021, 21:100972.

[40]
TANG Z T, LI C Y, XU G, et al. Effects of dietary glutathione on growth performance,muscle quality and lipid metabolism of hybrid crucian carp (Carassius auratus cuvieri ♀×Carassius auratus red var. ♂) fed a high-fat diet[J]. Reproduction and Breeding, 2023, 3(3):89-98.

[41]
HARIMANA Y, TANG X, XU P, et al. Effect of long-term moderate exercise on muscle cellularity and texture,antioxidant activities,tissue composition,freshness indicators and flavor characteristics in largemouth bass (Micropterus salmoides)[J]. Aquaculture, 2019, 510:100-108.

[42]
胡芬, 李小定, 熊善柏, 等. 5种淡水鱼肉的质构特性及与营养成分的相关性分析[J]. 食品科学, 2011, 32(11):69-73.

DOI

HU F, LI X D, XIONG S B, et al. Texture properties of freshwater fish and their correlation with nutritional components[J]. Food Science, 2011, 32(11):69-73. (in Chinese)

DOI

[43]
袁小琛, 陈范, 王光毅, 等. 暂养时间对鳙肌肉品质和营养价值的影响[J]. 淡水渔业, 2020, 50(6):83-91.

YUAN X C, CHEN F, WANG G Y, et al. Effects of purging time on meat quality and nutritional value of Aristichthys nobilis[J]. Freshwater Fisheries, 2020, 50(6):83-91. (in Chinese)

[44]
PERIAGO M J, AYALA M D, LÓPEZ-ALBORS O, et al. Muscle cellularity and flesh quality of wild and farmed sea bass,Dicentrarchus labrax L[J]. Aquaculture, 2005, 249(1/2/3/4):175-188.

[45]
LIN W L, ZENG Q X, ZHU Z W. Different changes in mastication between crisp grass carp (Ctenopharyngodon idellus C.et V) and grass carp (Ctenopharyngodon idellus) after heating:the relationship between texture and ultrastructure in muscle tissue[J]. Food Research International, 2009, 42(2):271-278.

[46]
WANG J S, ZHU Z Y, TIAN S H, et al. Dietary Lactobacillus casei K17 improves lipid metabolism,antioxidant response,and fillet quality of Micropterus salmoides[J]. Animals, 2021, 11(9):2564.

[47]
夏雨, 易华西, 范荣波, 等. 饲喂乳酸菌对凡纳滨对虾幼虾肉质的影响[J]. 中国水产科学, 2020, 27(1):74-81.

XIA Y, YI H X, FAN R B, et al. Effects of dietary lactic acid bacteria on the meat quality of juvenile Litopenaeus vannamei[J]. Journal of Fishery Sciences of China, 2020, 27(1):74-81. (in Chinese)

[48]
MOHANTY B P, MAHANTY A, GANGULY S, et al. Nutritional composition of food fishes and their importance in providing food and nutritional security[J]. Food Chemistry, 2019, 293:561-570.

DOI PMID

[49]
罗辉, 周剑, 叶华. 微生态制剂对鱼类肠道结构和消化酶活性的影响[J]. 水产科学, 2006, 25(2):105-108.

LUO H, ZHOU J, YE H. Effects of probiotics on structure and activity of digestive enzymes in intestine tracts in fish[J]. Fisheries Science, 2006, 25(2):105-108. (in Chinese)

[50]
WANG J S, ZHU Z Y, LI R, et al. Impact of supplementary Lactobacillus casei K17 on growth and gut health of largemouth bass Micropterus salmoides[J]. Aquaculture Reports, 2021, 20:100734.

[51]
王朝瑾, 赖雪萍, 康梅花, 等. 混合益生菌对鲫鱼生长和肌肉营养成分的影响[J]. 氨基酸和生物资源, 2011, 33(3):52-55.

WANG C J, LAI X P, KANG M H, et al. Effect of probiotics on the growth and muscle composition of crucian carp[J]. Amino Acids and Biotic Resources, 2011, 33(3):52-55. (in Chinese)

[52]
王亚玲, 王常安, 刘红柏, 等. 苏氨酸的鱼类营养生理研究进展[J]. 水产学杂志, 2021, 34(4):99-106.

WANG Y L, WANG C A, LIU H B, et al. Advances in nutritional physiology of dietary threonine in fish:a review[J]. Chinese Journal of Fisheries, 2021, 34(4):99-106. (in Chinese)

[53]
王劲松, 张昌桌, 陈燕, 等. 饲喂干酪乳杆菌K17对加州鲈鱼肌肉滋味的影响[J]. 食品工业科技, 2022, 43(12):46-53.

WANG J S, ZHANG C Z, CHEN Y, et al. Impact of supplement of Lactobacillus casei K17 on fillet tastes of largemouth bass Micropterus salmoides[J]. Science and Technology of Food Industry, 2022, 43(12):46-53. (in Chinese)

[54]
李琳娜, 王智勇, 王广军, 等. 添加微生态制剂和碳源对云斑尖塘鳢生长性能及肌肉品质的影响[J]. 安徽农业科学, 2023, 51(10):69-73.

LI L N, WANG Z Y, WANG G J, et al. Effects of adding the probiotics and carbon sources on growth performance and muscle quality of Oxyeleotris marmoratus[J]. Journal of Anhui Agricultural Sciences, 2023, 51(10):69-73. (in Chinese)

[55]
乔志刚, 张卫芳, 马龙. 2种微生态制剂对淇河鲫幼鱼摄食、生长和体成分的影响[J]. 水产科学, 2015, 34(1):26-31.

QIAO Z G, ZHANG W F, MA L. Effects of two probiotics on feeding,growth and body composition of juvenile Qihe crucian carp Carassius auratus[J]. Fisheries Science, 2015, 34(1):26-31. (in Chinese)

[56]
MEEX R C R, BLAAK E E. Mitochondrial dysfunction is a key pathway that links saturated fat intake to the development and progression of NAFLD[J]. Molecular Nutrition & Food Research, 2021, 65(1):1900942.

[57]
ROGERO M M, CALDER P C. Obesity,inflammation,Toll-like receptor 4 and fatty acids[J]. Nutrients, 2018, 10(4):432.

[58]
CALDER P C. Functional roles of fatty acids and their effects on human health[J]. Journal of Parenteral and Enteral Nutrition, 2015, 39(1 Suppl):18S-32S.

[59]
CHANG F Z, WANG Q, ZHANG Q, et al. Omega-3 polyunsaturated fatty acid inhibits the malignant progression of hepatocarcinoma by inhibiting the Wnt/β-catenin pathway[J]. European Review for Medical and Pharmacological Sciences, 2018, 22(14):4500-4508.

DOI PMID

[60]
ZHU X L, BI Z C, YANG C, et al. Effects of different doses of omega-3 polyunsaturated fatty acids on gut microbiota and immunity[J]. Food & Nutrition Research, 2021, 65:6263.

[61]
JOHN G, MOHAMED R R, KOLANCHINATHAN P, et al. Nutritional value of two bacterial strains Bacillus subtilis RCMB21 and Pseudomonas fluorescens RCMB39 as feed supplement for freshwater prawn Macrobrachium malcolmsonii[J]. Asian Journal of Animal and Veterinary Advances, 2018, 13(3):282-294.

[62]
HOSSAIN M K, ISHAK S D, IEHATA S, et al. Growth performance,fatty acid profile,gut,and muscle histo-morphology of Malaysian mahseer,Tor tambroides post larvae fed short-term host associated probiotics[J]. Aquaculture and Fisheries, 2024, 9(1):35-45.

[63]
ABD EL-HACK M E, EL-SAADONY M T, ELBESTAWY A R, et al. Undesirable odour substances (geosmin and 2-methylisoborneol) in water environment:sources,impacts and removal strategies[J]. Marine Pollution Bulletin, 2022, 178:113579.

[64]
LUKASSEN M B, SAUNDERS A M, SINDILARIU P D, et al. Quantification of novel geosmin-producing bacteria in aquaculture systems[J]. Aquaculture, 2017, 479:304-310.

[65]
周聃, 倪蒙, 刘梅, 等. 生态净养对去除大口黑鲈土腥味与提升营养成分的效果[J]. 水产学杂志, 2023, 36(3):96-103.

ZHOU D, NI M, LIU M, et al. Effect of ecological clean water holding on removal of earthy odor and improvement of nutrient compositions in largemouth bass Micropterus salmoides[J]. Chinese Journal of Fisheries, 2023, 36(3):96-103. (in Chinese)

[66]
ROHANI M F, ISLAM S M, HOSSAIN M K, et al. Probiotics,prebiotics and synbiotics improved the functionality of aquafeed:upgrading growth,reproduction,immunity and disease resistance in fish[J]. Fish & Shellfish Immunology, 2022, 120:569-589.

[67]
白利丹, 杨阳, 李晓伟, 等. 微生态制剂对锦鲤生长及水质的影响研究[J]. 安徽农业科学, 2014, 42(26):9051-9053.

BAI L D, YANG Y, LI X W, et al. Effect of probiotics on the growth of Cyprinus carpio and water quality[J]. Journal of Anhui Agricultural Sciences, 2014, 42(26):9051-9053. (in Chinese)

[68]
黄瑾, 熊邦喜, 陈洁, 等. 鱼类消化酶活性及其影响因素的研究进展[J]. 湖南农业科学, 2011(5):129-131,141.

HUANG J, XIONG B X, CHEN J, et al. Research advances in digestive enzyme of fish and its influencing factors[J]. Hunan Agricultural Sciences, 2011(5):129-131,141. (in Chinese)

[69]
李岩. 植物乳杆菌LP-S25复合诱变筛选及其在大口黑鲈养殖中的应用效果研究[D]. 硕士学位论文. 泰安: 山东农业大学, 2022.

LI Y.Screening of Lactobacillus plantarum LP-S 25 compound mutagenesis and screening mutagenic atrain application effect in largemouth bass[D]. Master's Thesis. Tai'an: Shandong Agricultural University, 2022. (in Chinese)

[70]
SEWAKA M, TRULLAS C, CHOTIKO A, et al. Efficacy of synbiotic Jerusalem artichoke and Lactobacillus rhamnosus GG-supplemented diets on growth performance,serum biochemical parameters,intestinal morphology,immune parameters and protection against Aeromonas veronii in juvenile red tilapia (Oreochromis spp.)[J]. Fish & Shellfish Immunology, 2019, 86:260-268.

[71]
陈南南. 饵料中添加芽孢杆菌对草鱼生长的影响及机理探讨[D]. 硕士学位论文. 杭州: 浙江大学, 2010.

CHEN N N. Study on effect of Bacillus on growth performance of grass carp and its mechanism[D]. Master's Thesis. Hangzhou: Zhejiang University, 2010. (in Chinese)

[72]
SUN Y Z, YANG H L, MA R L, et al. Effect of Lactococcus lactis and Enterococcus faecium on growth performance,digestive enzymes and immune response of grouper Epinephelus coioides[J]. Aquaculture Nutrition, 2012, 18(3):281-289.

[73]
孔雨昕, 徐晴, 田佳鑫, 等. 3种乳酸菌对乌鳢肠道消化酶、菌群、形态及紧密连接蛋白mRNA相对表达量的影响[J]. 吉林农业大学学报, 2022, 44(4):461-469.

KONG Y X, XU Q, TIAN J X, et al. Effects of three kinds of lactic acid bacteria on digestive enzymes,intestinal microbiota,intestinal morphology and relative expression levels of tight junction protein mRNA[J]. Journal of Jilin Agricultural University, 2022, 44(4):461-469. (in Chinese)

[74]
杜瑞玉. 酵母水解物和枯草芽孢杆菌在大口黑鲈饲料中的应用效果研究[D]. 硕士学位论文. 重庆: 西南大学, 2022.

DU R Y. Evaluation of yeast hydrolysate and Bacillus subtilis as feed additives in largemouth bass Micropterus salmoides[D]. Master's Thesis. Chongqing: Southwest University, 2022. (in Chinese)

[75]
樊英, 王晓璐, 于晓清, 等. 地衣芽孢杆菌对大泷六线鱼生长、肠道消化酶、血清非特异性免疫及抗病力的影响[J]. 渔业科学进展, 2021, 42(1):63-73.

FAN Y, WANG X L, YU X Q, et al. Effect of Bacillus licheniformis on growth,intestinal digestive enzyme activity,non-specific immunity,and resistance against Aeromonas salraonicida in the fat greenling (Hexagrammos otakii)[J]. Progress in Fishery Sciences, 2021, 42(1):63-73. (in Chinese)

[76]
徐晨, 李烨, 孙启睿, 等. 生物絮团养殖模式下益生菌添加对异育银鲫生长、消化酶活性及肠道组织结构的影响[J]. 中国水产科学, 2018, 25(5):1004-1011.

XU C, LI Y, SUN Q R, et al. Effects of probiotic addition on the growth performance,digestive enzyme activity,and intestinal morphology of gibel carp (Carassius auratus gibelio) cultured using biofloc technology[J]. Journal of Fishery Sciences of China, 2018, 25(5):1004-1011. (in Chinese)

[77]
ABID A, DAVIES S J, WAINES P, et al. Dietary synbiotic application modulates Atlantic salmon (Salmo salar) intestinal microbial communities and intestinal immunity[J]. Fish & Shellfish Immunology, 2013, 35(6):1948-1956.

[78]
崔广鑫, 孙娜, 王腾腾, 等. 蜡样芽孢杆菌YB1对大菱鲆幼鱼生长性能、肠道消化酶、肝脏抗氧化酶及肠道组织结构的影响[J]. 渔业科学进展, 2022, 43(1):97-105.

CUI G X, SUN N, WANG T T, et al. Effects of Bacillus cereus YB1 on growth performance,intestinal digestive enzymes,liver antioxidant enzymes,and intestinal tissue structure of juvenile turbot (Scophthalmus maximus)[J]. Progress in Fishery Sciences, 2022, 43(1):97-105. (in Chinese)

[79]
KOH A, DE VADDER F, KOVATCHEVA-DATCHARY P, et al. From dietary fiber to host physiology:short-chain fatty acids as key bacterial metabolites[J]. Cell, 2016, 165(6):1332-1345.

[80]
徐丹凤, 孙建琴. 短链脂肪酸对结肠功能的影响[J]. 营养健康新观察, 2009(2):7-10.

XU D F, SUN J Q. Effect of short chain fatty acids on colon function[J]. Nutrition Newsletter, 2009(2):7-10. (in Chinese)

[81]
NIMALAN N, SØRENSEN S L,

[82]
刘宇, 丁倩雯, 冉超, 等. 鱼虾肠道菌群代谢产物短链脂肪酸研究进展[J]. 生物技术通报, 2020, 36(2):58-64.

DOI

LIU Y, DING Q W, RAN C, et al. Research advances on short-chain fatty acids of metabolites of gut microbiota in aquatic animals[J]. Biotechnology Bulletin, 2020, 36(2):58-64. (in Chinese)

DOI

[83]
RINGOE E. Effects of dietary formate and acetate on growth and lipid digestibility in Arctic charr,Salvelinus alpinus (L.)[J]. Fiskeridirektoratets Skrifter Serie Ernaering, 1992, 5:17-24.

[84]
HASSAAN M S, WAFA M A, SOLTAN M A, et al. Effect of dietary organic salts on growth,nutrient digestibility,mineral absorption and some biochemical indices of Nile tilapia;Oreochromis niloticus L. fingerlings[J]. World Applied Sciences Journal, 2014, 29(1):47-55.

[85]
DE SCHRYVER P, SINHA A K, KUNWAR P S, et al. Poly-beta-hydroxybutyrate (PHB) increases growth performance and intestinal bacterial range-weighted richness in juvenile European sea bass,Dicentrarchus labrax[J]. Applied Microbiology and Biotechnology, 2010, 86(5):1535-1541.

[86]
MENG X L, WU S K, HU W P, et al. Clostridium butyricum improves immune responses and remodels the intestinal microbiota of common carp (Cyprinus carpio L.)[J]. Aquaculture, 2021, 530:735753.

[87]
张美玲, 单承杰, 杜震宇. 益生菌与鱼类肠道健康研究进展[J]. 水产学报, 2021, 45(1):147-157.

ZHANG M L, SHAN C J, DU Z Y. Research advances on probiotics and fish gut health[J]. Journal of Fisheries of China, 2021, 45(1):147-157. (in Chinese)

[88]
樊英, 叶海斌, 王晓璐, 等. 丁酸梭菌和凝结芽孢杆菌对虹鳟生长性能、肝功能及肠道菌群的影响[J]. 大连海洋大学学报, 2019, 34(2):198-203.

FAN Y, YE H B, WANG X L, et al. Effects of Clostridium butyricum and Bacillus coagulans on growth performance,hepatic function and intestinal microbiota in rainbow trout Oncorhynchus mykiss[J]. Journal of Dalian Fisheries University, 2019, 34(2):198-203. (in Chinese)

[89]
王颖. 黄鳝肠道菌群分析及益生菌应用的研究[D]. 硕士学位论文. 南昌: 江西农业大学, 2021.

WANG Y. Studies on intestinal flora of Monopterus albus and application of probiotics[D]. Master's Thesis. Nanchang: Jiangxi Agricultural University, 2021. (in Chinese)

[90]
钟立强, 王海骁, 王明华, 等. 不同饵料对大口黑鲈生长性能和肠道微生物的影响[J]. 水生生物学报, 2022, 46(11):1609-1617.

ZHONG L Q, WANG H X, WANG M H, et al. Different diets on growth performance and intestinal bacterial community of largemouth bass (Micropterus salmoides)[J]. Acta Hydrobiologica Sinica, 2022, 46(11):1609-1617. (in Chinese)

[91]
RAZIN S, YOGEV D, NAOT Y. Molecular biology and pathogenicity of mycoplasmas[J]. Microbiology and Molecular Biology Reviews, 1998, 62(4):1094-1156.

DOI PMID

[92]
刘滔. 中链脂肪酸单甘油酯对肉鸡生产性能和肉品质的影响及机制研究[D]. 博士学位论文. 杭州: 浙江大学, 2020.

LIU T. Effects and mechanisms of medium chain fatty acid monoglycerides on the productive performance and meat quality of broilers[D]. Ph.D.Thesis. Hangzhou: Zhejiang University, 2020. (in Chinese)

[93]
KASHINSKAYA E N, SIMONOV E P, IZVEKOVA G I, et al. Variability of composition of microbiota of gastrointestinal tract of perch Perca fluviatilis and Prussian carp Carassius gibelio during the vegetative season[J]. Journal of Ichthyology, 2021, 61(6):955-971.

[94]
RAMÍREZ C, CORONADO J, SILVA A, et al. Cetobacterium is a major component of the microbiome of giant Amazonian fish (Arapaima gigas) in Ecuador[J]. Animals, 2018, 8(11):189.

[95]
CHAPAGAIN P, ARIVETT B, CLEVELAND B M, et al. Analysis of the fecal microbiota of fast- and slow-growing rainbow trout (Oncorhynchus mykiss)[J]. BMC Genomics, 2019, 20(1):788.

DOI PMID

文章导航

/