研究论文

葛根素对脂多糖应激肉仔鸡生长性能、血清抗氧化和免疫指标以及肠道健康的影响

  • 龚番文 ,
  • 郅可欣 ,
  • 陈乐乐 ,
  • 李泽政 ,
  • 郜璐瑶 ,
  • 黄明海 ,
  • 符晨星 ,
  • 赵玉蓉 ,
  • 贺建华 , *
展开
  • 湖南农业大学动物科学技术学院,长沙 410125
*贺建华,教授,博士生导师,E-mail:

龚番文(1998—),男,江西九江人,硕士研究生,从事单胃动物营养研究。E-mail:

收稿日期: 2024-02-11

  网络出版日期: 2024-08-12

基金资助

国家重点研发计划(2023YFD1301200)

Effects of Puerarin on Growth Performance, Serum Antioxidant and Immune Indices and Intestinal Health of Broilers Challenged with Lipopolysaccharide

  • GONG Fanwen ,
  • ZHI Kexin ,
  • CHEN Lele ,
  • LI Zezheng ,
  • GAO Luyao ,
  • HUANG Minghai ,
  • FU Chenxing ,
  • ZHAO Yurong ,
  • HE Jianhua , *
Expand
  • College of Animal Science and Technology, Hunan Agricultural University, Changsha 410125, China
*professor, E-mail:

Received date: 2024-02-11

  Online published: 2024-08-12

摘要

本试验旨在研究饲粮中添加葛根素(PUE)对脂多糖(LPS)应激肉仔鸡生长性能、血清抗氧化和免疫指标、肠道形态及盲肠菌群的影响。选取288羽1日龄雄性黄羽肉鸡,随机分为4组,每组6个重复,每个重复12羽。对照组(CON组)和LPS应激组(LPS组)饲喂基础饲粮,葛根素组(PUE组)和葛根素+LPS应激组(PUEL组)在基础饲粮中添加750 mg/kg PUE。试验期20 d。分别在第16、18和20天,LPS组和PUEL组肉仔鸡腹腔注射500 μg/kg BW LPS,CON组和PUE组肉仔鸡腹腔注射等量无菌生理盐水。结果表明:1)LPS应激极显著降低了肉仔鸡平均日增重(ADG)(P<0.01),有降低平均日采食量(ADFI)(P=0.086)和提高料重比(F/G)(P=0.054)的趋势;饲粮中添加PUE有提高肉仔鸡ADG的趋势(P=0.089)。2)LPS应激极显著降低了肉仔鸡血清总超氧化物歧化酶(T-SOD)活性(P<0.01),显著降低了血清过氧化氢酶(CAT)活性(P<0.05),极显著提高了血清丙二醛(MDA)含量(P<0.01);饲粮中添加PUE显著提高了血清T-SOD活性(P<0.05),极显著降低了血清MDA含量(P<0.01)。3)LPS应激极显著提高了肉仔鸡血清白细胞介素-1β(IL-1β)、白细胞介素-2(IL-2)、肿瘤坏死因子-α(TNF-α)、免疫球蛋白A(IgA)和免疫球蛋白G(IgG)含量(P<0.01),极显著降低了血清白细胞介素-10(IL-10)含量(P<0.01);饲粮中添加PUE极显著降低了血清IL-1β和IL-2含量(P<0.01),显著降低了血清IgG含量(P<0.05)。饲粮中添加PUE与LPS应激对肉仔鸡血清IgA含量有极显著的交互作用(P<0.01),对血清IgG含量有显著的交互作用(P<0.05)。4)LPS应激极显著提高了肉仔鸡血清中D-乳酸(D-LA)和内毒素含量(P<0.01);饲粮中添加PUE与LPS应激对血清内毒素含量有显著的交互作用(P<0.05)。LPS应激显著降低了肉仔鸡回肠绒毛高度(VH)和绒隐比(V/C)(P<0.05)。5)LPS应激与饲粮中添加PUE改变了肉仔鸡盲肠菌群结构。在门水平上,LPS应激有降低盲肠厚壁菌门(Firmicutes)相对丰度的趋势(P=0.078)。在属水平上,LPS应激极显著降低了盲肠乳杆菌属(Lactobacillus)和norank_f_Eubacterium_coprostanoligenes_group相对丰度(P<0.01),显著提高了盲肠norank_f_norank_o_RF39和未定级梭菌纲vadinBB60群(norank_f_norank_o_Clostridia_vadinBB60_group)相对丰度(P<0.05);饲粮中添加PUE极显著提高了盲肠丁酸球菌属(Butyricicoccus)相对丰度(P<0.01)。饲粮中添加PUE与LPS应激对肉仔鸡盲肠norank_f_norank_o_RF39和丁酸球菌属相对丰度有极显著交互作用(P<0.01),对盲肠UCG-005相对丰度有显著交互作用(P<0.05)。综上所述,饲粮中添加750 mg/kg PUE可缓解机体氧化应激和炎症反应,改善肠道形态和菌群结构,在一定程度上缓解LPS应激对肉仔鸡造成的生长抑制和不利影响。

本文引用格式

龚番文 , 郅可欣 , 陈乐乐 , 李泽政 , 郜璐瑶 , 黄明海 , 符晨星 , 赵玉蓉 , 贺建华 . 葛根素对脂多糖应激肉仔鸡生长性能、血清抗氧化和免疫指标以及肠道健康的影响[J]. 动物营养学报, 2024 , 36(8) : 5050 -5066 . DOI: 10.12418/CJAN2024.430

Abstract

This experiment was conducted to investigate the effects of dietary puerarin (PUE) on growth performance, serum antioxidant and immune indices, intestinal morphology and cecal microbiota of broilers challenged with lipopolysaccharide (LPS). A total of 288 yellow-feathered male broilers of 1-day-old were randomly divided into 4 groups with 6 replicates per group and 12 broilers per replicate. Broilers in the control group (CON group) and LPS challenge group (LPS group) were fed a basal diet, and those in puerarin group (PUE group) and puerarin+LPS challenge group (PUEL group) were fed the basal diet supplemented with 750 mg/kg puerarin. The experiment period was 20 days. At 16, 18 and 20 days of age, broilers in LPS group and PUEL group were intraperitoneally injected with 500 μg/kg BW LPS, and broilers in CON group and PUE group were intraperitoneally injected with the same amount of sterile saline. The results showed as follows: 1) LPS challenge extremely significantly decreased the average daily gain (ADG) of broilers (P<0.01), tended to decrease the average daily feed intake (ADFI) (P=0.086) and increase the feed to gain ratio (F/G) (P=0.054). Dietary PUE tended to increase ADG of broilers (P=0.089). 2) LPS challenge extremely significantly decreased the total superoxide dismutase (T-SOD) activity in serum of broilers (P<0.01), significantly decreased the catalase (CAT) activity in serum (P<0.05), and extremely significantly increased the malondialdehyde (MDA) content in serum (P<0.01). Dietary PUE significantly increased the T-SOD activity in serum (P<0.05), and extremely significantly decreased the MDA content in serum (P<0.01). 3) LPS challenge extremely significantly increased the contents of interleukin-1β (IL-1β), interleukin-2 (IL-2), tumor necrosis factor-α (TNF-α), immunoglobulin A (IgA) and immunoglobulin G (IgG) in serum of broilers (P<0.01), and extremely significantly decreased the interleukin-10 (IL-10) content in serum (P<0.01). Dietary PUE extremely significantly decreased the contents of IL-1β and IL-2 in serum (P<0.01), and significantly decreased the IgG content in serum (P<0.05). Dietary PUE and LPS challenge showed an extremely significant interaction on the serum IgA content (P<0.01), and a significant interaction on the serum IgG content (P<0.05). 4) LPS challenge extremely significantly increased the contents of D-lactic acid (D-LA) and endotoxin in serum of broilers (P<0.01). Dietary PUE and LPS challenge showed a significant interaction on the serum endotoxin content (P<0.05). LPS challenge significantly decreased the ileal villus height (VH) and villus height to crypt depth ratio (V/C) of broilers (P<0.05). 5) LPS challenge and dietary PUE changed the cecal microbiota structure of broilers. At the phylum level, LPS challenge tended to decrease the Firmicutes relative abundance in cecum (P=0.078). At the genus level, LPS challenge extremely significantly decreased the relative abundances of Lactobacillus and norank_f_Eubacterium_coprostanoligenes_group in cecum (P<0.01), and significantly increased the relative abundances of norank_f_norank_o_RF39 and norank_f_norank_o_Clostridia_vadinBB60_group in cecum (P<0.05). Dietary PUE significantly increased the Butyricicoccus relative abundance in cecum (P<0.05). Dietary PUE and LPS challenge showed an extremely significant interaction on the relative abundances of norank_f_norank_o_RF39 and Butyricicoccus in cecum (P<0.01), and a significant interaction on the UCG-005 relative abundance in cecum (P<0.05). In conclusion, dietary 750 mg/kg PUE can alleviate oxidative stress and inflammatory response, improve intestinal morphology and cecal microbiota structure, alleviate growth inhibition and adverse effects caused by LPS challenge to a certain extent.

免疫应激是指动物机体在抗原或应激源的频繁刺激下,免疫系统不断被激活,从而引发的非特异性适应反应[1]。现代集约化养殖模式中,肉鸡常面临高密度养殖、病原微生物感染和热应激等应激源刺激,从而产生免疫应激,导致肠道屏障受损以及肠道炎症的发生,严重危害动物的肠道健康[2-4]。肠道形态、肠道通透性、肠道免疫功能以及肠道微生物组成是评价家禽肠道健康的重要指标[5]。肠道是机体最大的消化吸收场所和免疫器官,肠道健康失衡会降低家禽对营养物质的消化吸收[6]。因而寻找一种绿色安全的饲料添加剂用于保护肉鸡机体和肠道健康,对于提高动物生长性能和家禽养殖业的经济效益具有重要意义。
葛根素(puerarin,PUE)是从药食同源植物葛根中提取的一种天然异黄酮类物质,具有抗氧化、抗炎以及调节脂质代谢等多种生物学功能,在畜禽生产中具有较广阔的应用前景[7-9]。据报道,PUE通过提高肠道紧密连接蛋白表达,增强肠道抗氧化能力,调节肠道菌群结构,在维护动物肠道健康方面发挥积极的作用[10-12]。汪纪仓等[13]研究发现,饲粮中添加0.8 g/kg PUE可提高肉鸡抗氧化能力。研究报道,肉鸡饲粮中添加750 mg/kg PUE可以降低机体炎症反应,提高肠道抗氧化能力,缓解氧化大豆油诱导的免疫器官和肠道屏障损伤[14-15]。Du等[16]研究发现,饲粮中添加800 mg/kg PUE可提高产蛋后期蛋鸡的产蛋性能和蛋品质,改善肠道形态和肠道抗氧化能力。此外,饲粮中添加PUE还可缓解大肠杆菌和沙门氏菌攻毒对肉鸡产生的不良影响[17-18]。然而,目前关于PUE对肉鸡在免疫应激状态下的研究较少,尤其是对于肠道健康方面。因此,本研究通过腹腔注射脂多糖(LPS)构建免疫应激模型,旨在探讨PUE对免疫应激状态下肉仔鸡生长性能、血清抗氧化和免疫指标以及肠道健康的影响,为PUE在肉鸡健康生产中的应用提供理论依据。

1 材料与方法

1.1 试验材料

葛根素由陕西省某公司提供,分子式为C21H20O9,化学名为8-β-D-葡萄吡喃糖-4',7-二羟基异黄酮,纯度≥98%。LPS(血清型O55:B5,货号L2880)购自Sigma公司。

1.2 试验动物和试验设计

试验采取2(0或750 mg/kg PUE)×2(是否LPS应激)双因素试验设计,选取288羽健康的1日龄、平均初重为(32.63±0.07) g的黄羽肉仔鸡公雏(品种为黄花鸡,生长速度介于中速和快速之间),随机分为4组,每组设6个重复,每个重复12羽。对照组(CON组)和LPS应激组(LPS组)饲喂基础饲粮;葛根素组(PUE组)和葛根素+LPS应激组(PUEL组)在基础饲粮中添加750 mg/kg葛根素。PUE添加剂量参考文献[13-15]。试验期20 d,包括应激前期(1~15日龄)和应激期(16~20日龄)。于试验第16、18和20天时,对LPS组和PUEL组肉仔鸡腹腔注射500 μg/kg BW LPS,对CON组和PUE组肉仔鸡腹腔注射等量的无菌生理盐水,LPS给药剂量和方法参照An等[19]的研究。

1.3 试验饲粮

基础饲粮参照《黄羽肉鸡营养需要量》(NY/T 3645—2020)[20]配制成粉状饲料,其组成鸡营养水平见表1。饲粮中粗蛋白质、钙和总磷含量分别参照《饲料中粗蛋白的测定 凯氏定氮法》(GB/T 6432—2018)[21]、《饲料中钙的测定》(GB/T 6436—2018)[22]和《饲料中总磷的测定 分光光度法》(GB/T 6437—2018)[23]的方法进行测定。饲粮代谢能水平以及有效磷和氨基酸含量参照《中国饲料成分及营养价值表(2020年第31版)》[24]进行计算。
表1 基础饲粮组成及营养水平(风干基础)

Table 1 Composition and nutrient levels of the basal diet (air-dry basis) %

项目Items 含量Content
原料Ingredients
玉米Corn 56.78
豆粕Soybean meal 29.00
玉米蛋白粉Corn gluten meal 5.00
麦麸Wheat bran 2.60
大豆油Soybean oil 2.20
磷酸氢钙CaHPO4 1.30
石粉Limestone 1.20
氯化钠NaCl 0.30
L-赖氨酸L-Lys 0.54
DL-蛋氨酸DL-Met 0.18
氯化胆碱Choline chloride 0.10
预混料Premix1) 0.80
合计Total 100.00
营养水平Nutrient levels2)
代谢能ME/ (MJ/kg) 12.25
粗蛋白质CP 21.16
钙Ca 0.92
有效磷AP 0.43
总磷TP 0.53
赖氨酸Lys 1.20
蛋氨酸Met 0.54
蛋氨酸+胱氨酸Met+Cys 0.88
苏氨酸Thr 0.77
色氨酸Trp 0.21

1)预混料为每千克饲粮提供 The premix provided the following per kg of the diet:VA 12 000 IU,VD3 4 000 IU,VE 20 IU,VK 10 mg,VB1 4.0 mg,VB2 8.0 mg,VB66.0 mg,VB12 0.02 mg,叶酸 folic acid 1.5 mg,烟酸 nicotinic acid 40 mg,泛酸 pantothenic acid 15 mg,生物素 biotin 0.2 mg,Mn 90 mg,Fe 90 mg,Zn 60 mg,Cu 15 mg,Se 0.20 mg,I 0.80 mg。

2)粗蛋白质、钙和总磷含量为实测值,其余为计算值。CP, Ca and TP were measured values, while the others were calculated values.

1.4 饲养管理

本试验采用网床平养,对鸡舍全方位消毒清洁后,将肉仔鸡饲养在同一环境条件下。鸡舍第1周温度保持在33~34 ℃,随后每隔1周温度降低2~3 ℃,保持自然通风。所有肉仔鸡均自由采食和饮水,鸡群按正常免疫程序进行免疫接种。

1.5 样品采集与处理

在试验第21天,从每个重复中抽取1只接近平均体重的肉仔鸡(禁食12 h,断料不断水),翅静脉采血5 mL于采血管中,先室温静置30 min,待血清析出后于4 ℃、999×g下离心15 min分离血清,再保存于-80 ℃冰箱中。随后对肉鸡进行屠宰,剖开腹腔,迅速分离并采集十二指肠、空肠和回肠的中间部位约1 cm的肠段,用0.9%生理盐水冲洗后置于4%多聚甲醛溶液中进行固定。

1.6 测定指标及方法

1.6.1 生长性能

分别于1、15和20日龄对每个重复的肉仔鸡进行空腹称重,每天记录各个重复的采食量。计算应激前期(1~15日龄)和应激期(16~20日龄)各重复的平均日增重(ADG)、平均日采食量(ADFI)和料重比(F/G)。

1.6.2 血清抗氧化指标

按照试剂盒(南京建成生物工程研究所)说明书的方法测定血清抗氧化指标,包括:血清谷胱苷肽过氧化物酶(GSH-Px)、总超氧化物歧化酶(T-SOD)和过氧化氢酶(CAT)活性以及丙二醛(MDA)含量。

1.6.3 血清免疫和肠道通透性指标

按照酶联免疫吸附试验(ELISA)试剂盒(江苏酶免实业有限公司)说明书的方法测定血清免疫指标和肠道通透性指标,包括:血清白细胞介素-1β(IL-1β)、白细胞介素-2(IL-2)、白细胞介素-10(IL-10)、肿瘤坏死因子-α(TNF-α)、免疫球蛋白A(IgA)、免疫球蛋白M(IgM)以及D-乳酸(D-lactic acid,D-LA)和内毒素(endotoxin)含量。

1.6.4 肠道黏膜形态

将十二指肠、空肠和回肠肠段放入4%多聚甲醛组织固定液后,经冲水、二甲苯透膜、石蜡包埋、切片和苏木精-伊红(HE)染色等步骤后,在40倍光学显微镜视野下随机选取多个绒毛和隐窝的采集图像,测量绒毛高度(villus height,VH)和隐窝深度(crypt depth,CD),并计算绒隐比(V/C)。

1.6.5 盲肠菌群

收集盲肠内容物于无菌冻存管中,液氮速冻后保存于-80 ℃冰箱,再由上海美吉生物医药科技有限公司对盲肠内容物进行16S rRNA测序和微生物多样性分析。

1.7 数据处理与分析

所有数据经Excel 2021整理后,采用SPSS 26.0软件进行单因素方差分析(one-way ANOVA),当差异显著时,采用Duncan氏法进行多重比较;然后,进一步采用一般线性模型单变量双因素方差分析,分析添加PUE和LPS应激这2个主效应以及两者交互作用的影响。结果以平均值和均值标准误(SEM)表示,P<0.05表示差异显著,P<0.01表示差异极显著,0.05≤P<0.10表示差异有显著趋势。

2 结果与分析

2.1 PUE对LPS应激肉仔鸡生长性能的影响

表2可知,1~15日龄,饲粮中添加PUE对肉仔鸡ADG、ADFI和F/G均无显著影响(P>0.05)。16~20日龄,LPS应激极显著降低了肉仔鸡ADG(P<0.01),有降低ADFI(P=0.086)以及提高F/G(P=0.054)的趋势;饲粮中添加PUE有提高肉仔鸡ADG的趋势(P=0.089)。饲粮中添加PUE与LPS应激对肉仔鸡生长性能无显著交互作用(P>0.05)。多重比较结果显示,16~20日龄,与CON组相比,LPS组肉仔鸡ADG显著降低(P<0.05)。
表2 PUE对LPS应激肉仔鸡生长性能的影响

Table 2 Effects of PUE on growth performance of broilers challenged with LPS

项目
Items
组别Groups 均值
标准误
SEM
PP-value
CON LPS PUE PUEL PUE LPS PUE×LPS
1~15日龄1 to 15 days of age
平均日增重ADG/(g/d) 15.76 15.56 15.18 15.58 0.149 0.422
平均日采食量ADFI/(g/d) 25.46 25.03 25.01 25.25 0.201 0.862
料重比F/G 1.61 1.60 1.64 1.59 0.016 0.713
16~20日龄16 to 20 days of age
平均日增重ADG/(g/d) 31.19ab 27.78c 32.13a 29.54bc 0.582 0.089 0.001 0.585
平均日采食量ADFI/(g/d) 52.47 48.40 53.13 51.76 0.800 0.198 0.086 0.381
料重比F/G 1.68 1.74 1.66 1.75 0.020 0.339 0.054 0.780

PUE:添加PUE效应;LPS:LPS应激效应;PUE×LPS:添加PUE与LPS应激的交互作用。同行数据肩标无字母或相同字母表示差异不显著(P>0.05),不同小写字母表示差异显著(P<0.05)。下同表。

PUE: effect of dietary PUE; LPS: effect of LPS challenge; PUE×LPS: interaction of dietary PUE and LPS challenge. In the same row, values with no letter or the same letter superscripts mean no significant difference (P>0.05), while with different small letter superscripts mean significant difference (P<0.05). The same as below.

2.2 PUE对LPS应激肉仔鸡血清抗氧化指标的影响

表3可知,LPS应激极显著降低了肉仔鸡血清T-SOD活性(P<0.01),显著降低了血清CAT活性(P<0.05),极显著提高了血清MDA含量(P<0.01);饲粮中添加PUE显著提高了血清T-SOD活性(P<0.05),有提高血清CAT活性的趋势(P=0.076),极显著降低了血清MDA含量(P<0.01)。饲粮中添加PUE与LPS应激对肉仔鸡血清MDA含量有显著交互作用的趋势(P=0.063)。多重比较结果显示,与LPS组相比,PUEL组肉仔鸡血清MDA含量显著降低(P<0.05)。
表3 PUE对LPS应激肉仔鸡血清抗氧化指标的影响

Table 3 Effects of PUE on serum antioxidant indices of broilers challenged with LPS

项目
Items
组别Groups 均值
标准误
SEM
PP-value
CON LPS PUE PUEL PUE LPS PUE×LPS
谷胱甘肽过氧化物酶GSH-Px/(U/mL) 607.21 603.27 603.54 608.52 20.530 0.770 0.846 0.108
总超氧化物歧化酶T-SOD /(U/mL) 62.63ab 48.92c 67.92a 55.86bc 1.522 0.028 <0.001 0.752
过氧化氢酶CAT/(U/mL) 29.85ab 25.79b 34.76a 29.00ab 1.211 0.076 0.035 0.698
丙二醛MDA/(nmol/mL) 5.77bc 8.65a 5.26c 6.54b 0.330 0.004 <0.001 0.063

2.3 PUE对LPS应激肉仔鸡血清免疫指标的影响

表4可知,LPS应激极显著提高了肉仔鸡血清IL-1β、IL-2、TNF-α、IgA和IgG含量(P<0.01),极显著降低了血清IL-10含量(P<0.01);饲粮中添加PUE极显著降低了血清中IL-1β和IL-2含量(P<0.01),显著降低了血清IgG含量(P<0.05)。饲粮中添加PUE与LPS应激对肉仔鸡血清IgA含量存在极显著交互作用(P<0.01),对血清IgG含量存在显著交互作用(P<0.05),对血清IL-10含量有显著交互作用的趋势(P=0.077)。多重比较结果显示,与LPS组相比,PUEL组肉仔鸡血清IL-1β、IL-2、IgA和IgG含量显著降低(P<0.05)。
表4 PUE对LPS应激肉仔鸡血清免疫指标的影响

Table 4 Effects of PUE on serum immune indices of broilers challenged with LPS

项目
Items
组别Groups 均值
标准误
SEM
PP-value
CON LPS PUE PUEL PUE LPS PUE×LPS
白细胞介素-1β IL-1β/(pg/mL) 27.44c 45.15a 25.05c 39.51b 1.831 0.004 <0.001 0.209
白细胞介素-2 IL-2/(pg/mL) 93.76c 121.47a 87.35c 109.58b 3.049 0.003 <0.001 0.313
肿瘤坏死因子-α TNF-α/(pg/mL) 7.20 10.94a 6.84b 9.55a 0.429 0.114 <0.001 0.341
白细胞介素-10 IL-10/(pg/mL) 84.84a 55.26b 83.03a 61.84b 2.891 0.302 <0.001 0.077
免疫球蛋白A IgA/(g/L) 15.94c 25.54a 18.20c 21.17b 0.834 0.204 <0.001 <0.001
免疫球蛋白G IgG/(g/L) 15.37c 24.29a 15.30c 20.24b 0.868 0.013 <0.001 0.016

2.4 PUE对LPS应激肉仔鸡血清肠道通透性指标的影响

表5可知,LPS应激极显著提高了肉仔鸡血清D-LA和内毒素含量(P<0.01);饲粮中添加PUE有降低血清内毒素含量的趋势(P=0.074)。饲粮中添加PUE与LPS应激对肉鸡血清内毒素含量有显著交互作用(P<0.05)。多重比较结果显示,与LPS组相比,PUEL组肉仔鸡血清内毒素含量显著降低(P<0.05)。
表5 PUE对LPS应激肉仔鸡血清肠道通透性指标的影响

Table 5 Effects of PUE on serum intestinal permeability indices of broilers challenged with LPS

项目
Items
组别Groups 均值
标准误
SEM
PP-value
CON LPS PUE PUEL PUE LPS PUE×LPS
D-乳酸D-LA/(ng/mL) 47.81b 60.24a 47.10b 57.40a 1.314 0.132 <0.001 0.356
内毒素Endotoxin/(EU/L) 0.27c 0.42a 0.28c 0.34b 0.016 0.074 <0.001 0.026

2.5 PUE对LPS应激肉仔鸡肠道黏膜形态的影响

表6可知,LPS应激显著降低了肉仔鸡回肠VH和V/C(P<0.05),有降低十二指肠V/C(P=0.061)和空肠VH(P=0.057)的趋势;饲粮中添加PUE有提高回肠VH(P=0.082)和V/C(P=0.073)的趋势。饲粮中添加PUE与LPS应激对肉仔鸡十二指肠、空肠和回肠黏膜形态指标均无显著交互作用(P>0.05)。多重比较结果显示,与LPS组相比,PUEL组肉仔鸡回肠VH显著提高(P<0.05)。
表6 PUE对LPS应激肉仔鸡龄肠道黏膜形态的影响

Table 6 Effects of PUE on intestinal mucosa morphology of broilers challenged with LPS

项目
Items
组别Groups 均值
标准误
SEM
PP-value
CON LPS PUE PUEL PUE LPS PUE×LPS
十二指肠Duodenum
绒毛高度Villus height/μm 708.55 634.35 714.67 654.75 39.270 0.739 0.103 0.858
隐窝深度Crypt depth/μm 109.28 116.63 108.99 100.11 8.254 0.320 0.927 0.337
绒隐比V/C 6.57 5.63 6.85 5.97 0.456 0.510 0.061 0.950
空肠Jejunum
绒毛高度Villus height/μm 567.49 524.93 593.58 520.46 28.619 0.710 0.057 0.599
隐窝深度Crypt depth/μm 121.01 109.09 106.08 108.70 9.243 0.417 0.620 0.441
绒隐比V/C 4.77 4.93 5.75 4.98 0.420 0.231 0.473 0.284
回肠Ileum
绒毛高度Villus height/μm 497.72a 410.71b 502.42a 480.02a 12.144 0.082 0.014 0.125
隐窝深度Crypt depth/μm 101.99 96.37 88.51 100.26 2.615 0.359 0.555 0.105
绒隐比V/C 4.89ab 4.39b 5.78a 4.78ab 0.190 0.073 0.040 0.473

2.6 PUE对LPS应激肉仔鸡盲肠菌群的影响

2.6.1 盲肠菌群操作分类单元(OTU)分析
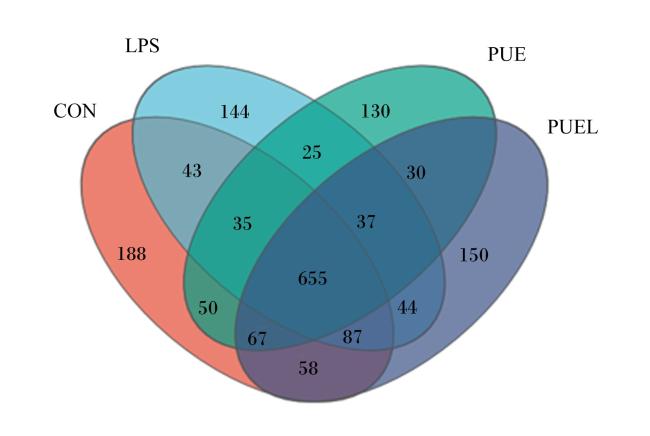
图1所示,在97%相似性水平下,各组肉仔鸡盲肠菌群共有OTU数目为655个。其中,CON组盲肠菌群共有OTU数目为1 183个,特有OTU数目为188个;LPS组盲肠菌群共有OTU数目为1 060个,特有OTU数目为144个;PUE组盲肠菌群共有OTU数目为1 029个,特有OTU数目130个;PUEL组盲肠菌群共有OTU数目1 128个,特有OTU数目150个。上述结果说明,LPS应激和饲粮中添加PUE对肉仔鸡盲肠菌群结构产生了一定的影响。
图1 肉仔鸡盲肠菌群OTU的韦恩图

CON:对照组 control group;LPS:LPS应激组 LPS challenge group;PUE:葛根素组 puerarin group;PUEL:葛根素+LPS应激组 puerarin+LPS challenge group。

Fig.1 Venn diagram of OTU of cecal microbiota of broilers

2.6.2 盲肠菌群α多样性分析

表7可知,LPS应激有降低肉仔鸡盲肠菌群Shannon指数的趋势(P=0.051);饲粮中添加PUE对盲肠菌群α多样性指数均无显著影响(P>0.05)。饲粮中添加PUE与LPS应激对肉仔鸡盲肠菌群Ace指数、Chao1指数和Simpson指数均无显著交互作用(P>0.05),对Shannon指数有显著交互作用的趋势(P=0.081)。
表7 PUE对LPS应激肉仔鸡盲肠菌群α多样性的影响

Table 7 Effects of PUE on α diversity of cecal microbiota of broilers challenged with LPS

项目
Items
组别Groups 均值
标准误
SEM
PP-value
CON LPS PUE PUEL PUE LPS PUE×LPS
Ace指数Ace index 716.33 622.57 626.38 670.21 17.788 0.245 0.205 0.162
Chao1指数Chao1 index 702.30 584.76 623.47 621.50 18.866 0.561 0.109 0.121
Shannon指数Shannon index 4.07 3.44 3.76 3.72 0.083 0.264 0.051 0.081
Simpson指数Simpson index 0.07 0.12 0.07 0.08 0.009 0.372 0.129 0.203

2.6.3 盲肠菌群β多样性分析

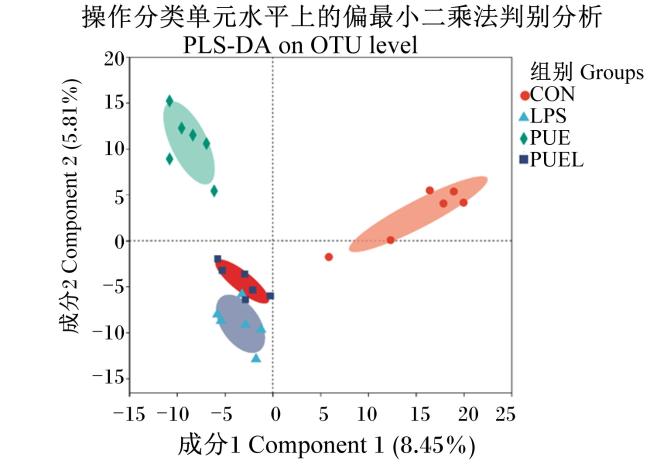
图2所示,基于OTU的偏最小二乘法判别分析(PLS-DA)结果,4个组肉仔鸡盲肠菌群结构差异明显。其中,LPS组和PUEL组的OTU聚类较近,CON组和PUE组的OTU聚类较远,说明饲粮中添加PUE与LPS应激均引起肉仔鸡盲肠菌群结构发生改变,并且LPS组和PUEL组样本间盲肠菌群结构更相似。
图2 PUE对LPS应激肉仔鸡盲肠菌群β多样性的影响

Fig.2 Effects of PUE on β diversity of cecal microbiota of broilers challenged with LPS

2.6.4 盲肠菌群在门水平上的组成分析

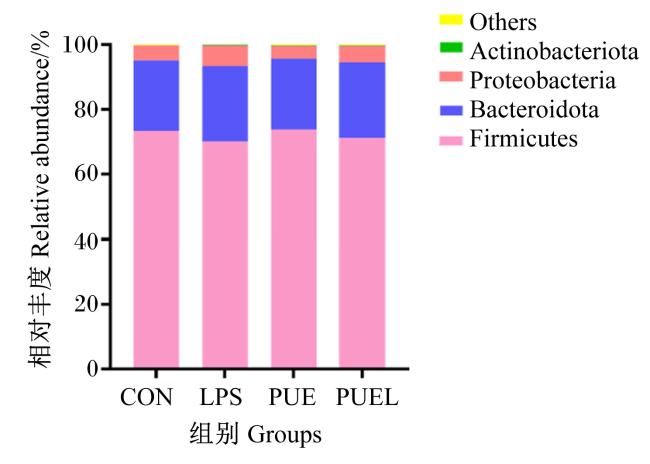
图3表8可知,在门水平上,LPS应激有降低肉仔鸡盲肠厚壁菌门(Firmicutes)相对丰度的趋势(P=0.078),对盲肠拟杆菌门(Bacteroidota)、变形菌门(Proteobacteria)和放线菌门(Actinobacteriota)相对丰度均无显著影响(P>0.05)。饲粮中添加PUE与LPS应激对肉仔鸡盲肠菌群在门水平上的相对丰度均无显著交互作用(P>0.05)。
图3 PUE对LPS应激肉仔鸡盲肠菌群在门水平上相对丰度的影响

Others:其他;Actinobacteriota:放线菌门;Proteobacteria:变形菌门;Bacteroidota:拟杆菌门;Firmicutes:厚壁菌门。

Fig.3 Effects of PUE on relative abundance of cecal microbiota at phylum level of broilers challenged with LPS

表8 PUE对LPS应激肉仔鸡盲肠菌群在门水平上相对丰度的影响

Table 8 Effects of PUE on relative abundance of cecal microbiota at phylum level of broilers challenged with LPS %

项目
Items
组别Groups 均值
标准误
SEM
PP-value
CON LPS PUE PUEL PUE LPS PUE×LPS
厚壁菌门Firmicutes 73.41 70.21 73.78 71.27 1.537 0.646 0.078 0.825
拟杆菌门Bacteroidota 21.71 23.15 21.86 23.29 1.060 0.893 0.191 0.998
变形菌门Proteobacteria 4.62 6.44 4.02 5.10 0.152 0.369 0.185 0.734
放线菌门Actinobacteriota 0.14 0.15 0.19 0.09 0.040 0.935 0.285 0.190
其他Others 0.12 0.06 0.16 0.24 0.156 0.490 0.946 0.630

2.6.5 盲肠菌群在属水平上的组成分析

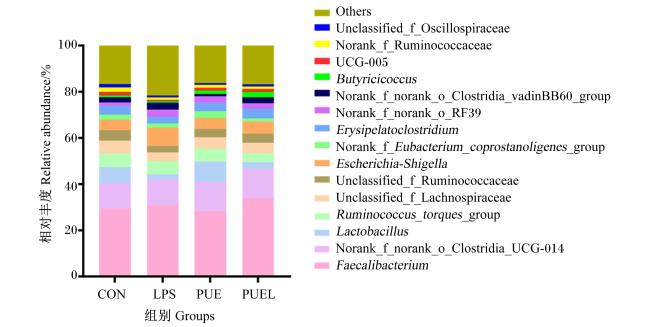
在属水平上,对相对丰度大于1%的菌属进行统计分析,分别是粪杆菌属(Faecalibacterium)、未定级梭菌纲UCG-014(norank_f_norank_o_Clostridia_UCG-014)、乳杆菌属(Lactobacillus)、瘤胃球菌属扭链群(Ruminococcus_torques_group)、未分类毛螺菌科(unclassified_f_Lachnospiraceae)、未分类瘤胃球菌科(unclassified_f_Ruminococcaceae)、埃希氏-志贺氏菌属(Escherichia-Shigella)、norank_f_Eubacterium_coprostanoligenes_group、Erysipelatoclostridium、norank_f_norank_o_RF39、未定级梭菌纲vadinBB60群(norank_f_norank_o_Clostridia_vadinBB60_group)、丁酸球菌属(Butyricicoccus)、UCG-005、未定级瘤胃球菌科(norank_f_Ruminococcaceae)和未分类颤螺菌科(unclassified_f_Oscillospiraceae)。如图4表9所示,LPS应激极显著降低了肉仔鸡盲肠乳杆菌属和norank_f_Eubacterium_coprostanoligenes_group相对丰度(P<0.01),显著降低了盲肠未定级瘤胃球菌科相对丰度(P<0.05),有降低盲肠UCG-005相对丰度的趋势(P=0.088);LPS应激显著提高了盲肠norank_f_norank_o_RF39和未定级梭菌纲vadinBB60群相对丰度(P<0.05),有提高盲肠埃希氏-志贺氏菌属相对丰度的趋势(P=0.051);饲粮中添加PUE极显著提高了盲肠丁酸球菌属相对丰度(P<0.01),有降低盲肠未定级梭菌纲vadinBB60群相对丰度的趋势(P=0.070)。饲粮中添加PUE与LPS应激对肉仔鸡盲肠norank_f_norank_o_RF39和丁酸球菌属相对丰度有极显著交互作用(P<0.01),对盲肠UCG-005相对丰度有显著交互作用(P<0.05),对盲肠norank_f_Eubacterium_coprostanoligenes_group相对丰度有显著交互作用的趋势(P=0.091)。多重比较结果显示,与CON组相比,PUE组肉仔鸡盲肠norank_f_norank_o_RF39和丁酸球菌属相对丰度显著提高(P<0.05);与LPS组相比,PUEL组盲肠丁酸球菌属相对丰度显著提高(P<0.05)。
图4 PUE对LPS应激肉仔鸡盲肠菌群在属水平上相对丰度的影响

Others:其他;Unclassified_f_Oscillospiraceae:未分类颤螺菌科;Norank_f_Ruminococcaceae:未定级瘤胃球菌科;Butyricicoccus:丁酸球菌属;Norank_f_norank_o_Clostridia_vadinBB60_group:未定级梭菌纲vadinBB60群;Escherichia-Shigella:埃希氏-志贺氏菌属;Unclassified_f_Ruminococcaceae:未分类瘤胃球菌科;Unclassified_f_Lachnospiraceae:未分类毛螺菌科;Ruminococcus_torques_group:瘤胃球菌属扭链群;Lactobacillus:乳杆菌属;Norank_f_norank_o_Clostridia_UCG-014:未定级梭菌纲UCG-014;Faecalibacterium:粪杆菌属。

Fig.4 Effects of PUE on relative abundance of cecal microbiota at genus level of broilers challenged with LPS

表9 PUE对LPS应激肉仔鸡盲肠菌群在属水平上相对丰度的影响

Table 9 Effects of PUE on relative abundance of cecal microbiota at genus level of broilers challenged with LPS

项目
Items
组别Groups 均值
标准误
SEM
PP-value
CON LPS PUE PUEL PUE LPS PUE×LPS
粪杆菌属Faecalibacterium 29.75 30.81 28.26 34.03 1.780 0.323 0.317 0.487
未定级梭菌纲UCG-014
Norank_f_norank_o_Clostridia_UCG-014
11.12 11.29 12.64 12.60 1.865 0.457 0.973 0.959
乳杆菌属Lactobacillus 6.94ab 2.33b 8.88a 2.82b 0.631 0.313 0.001 0.587
瘤胃球菌属扭链群
Ruminococcus_torques_group
5.94 5.57 5.60 3.87 0.700 0.161 0.148 0.339
未分类毛螺菌科
Unclassified_f_Lachnospiraceae
5.56 3.77 4.89 4.64 0.353 0.888 0.160 0.284
未分类瘤胃球菌科
Unclassified_f_Ruminococcaceae
4.41 2.90 3.65 3.88 0.407 0.898 0.455 0.314
埃希氏-志贺氏菌属
Escherichia-Shigella
4.62 7.91 4.66 5.26 0.939 0.179 0.051 0.168
Norank_f_Eubacterium_
coprostanoligenes_group
2.19ab 1.77b 3.03a 1.35b 0.350 0.554 0.007 0.091
Erysipelatoclostridium 3.90 2.98 3.68 4.12 0.569 0.429 0.679 0.245
Norank_f_norank_o_RF39 1.36b 3.03a 2.74a 2.44a 0.255 0.137 0.014 0.001
未定级梭菌纲vadinBB60群
Norank_f_norank_o_Clostridia_
vadinBB60_group
2.22ab 3.01a 0.96b 2.55a 0.448 0.070 0.015 0.380
丁酸球菌属Butyricicoccus 0.84c 0.58c 1.53b 2.30a 0.154 <0.001 0.115 0.003
UCG-005 1.59a 0.64b 1.14ab 1.29ab 0.223 0.665 0.088 0.023
未定级瘤胃球菌科
Norank_f_Ruminococcaceae
1.93a 1.09b 1.36ab 1.16b 0.231 0.293 0.036 0.184
未分类颤螺菌科
Unclassified_f_Oscillospiraceae
1.32 0.79 0.79 0.85 0.227 0.315 0.309 0.201
其他Others 15.41 20.74 15.48 16.53 3.810 0.594 0.412 0.581

3 讨论

3.1 PUE对LPS应激肉仔鸡生长性能的影响

机体过度的炎症反应和氧化应激通常会抑制动物生长。研究发现,LPS应激通过抑制采食中枢的局部兴奋性,导致动物食欲不振、采食量降低;同时增强体内分解代谢,使营养物质重新分配,将更多的能量用于抵抗应激,造成动物生长性能的降低[25]。Li等[26]和Fan等[27]研究报道,肉仔鸡腹腔注射LPS后,引起机体炎症反应和氧化损伤,导致生长性能显著降低。本试验中,LPS应激极显著降低了肉仔鸡ADG,有降低ADFI以及提高F/G的趋势,这与上述研究结果基本一致。
以往研究表明,PUE是一种潜在的可用于缓解家禽免疫应激的天然植物多酚[14-15]。汪纪仓等[13]研究发现,饲粮中添加0.4、0.8和1.6 g/kg的PUE可以改善肉鸡的抗氧化能力,但对生长性能无显著影响。余应梅等[28]研究发现,饲粮中添加PUE可显著提高肉鸡生长后期的ADFI。Lu等[29]研究发现,PUE可以改善沙门氏菌感染引起的氨基酸和脂质代谢异常,提高肉仔鸡生长性能。本试验中,在LPS应激前期,饲粮中添加PUE对肉仔鸡的生长性能无显著影响。在LPS应激期,在非应激条件下饲粮中添加PUE对肉仔鸡生长性能有改善作用,但效果不显著;在应激条件下饲粮中添加PUE有提高肉仔鸡ADG的趋势,在一定程度上缓解了应激引起的生长抑制。这可能与PUE具有抗氧化和抗炎特性有关,改善了应激条件下机体的健康状况。因此,本试验进一步探讨了PUE对LPS应激肉仔鸡抗氧化能力和免疫功能的影响。

3.2 PUE对LPS应激肉仔鸡血清抗氧化指标的影响

正常生理状况下,由GSH-Px、T-SOD和CAT等抗氧化酶组成的酶促系统与非酶促系统通过清除活性氧自由基,减少脂质过氧化反应,使机体免受氧化应激[30]。MDA是脂质过氧化的终末产物,其含量可以反映机体的氧化状态[31]。以往研究表明,LPS应激会造成肉鸡血清[32]、肝脏[33]和肠道[34]等组织器官中抗氧化酶活性的降低,引起氧化应激。本试验中,LPS应激引起肉仔鸡血清MDA含量显著升高,血清T-SOD和CAT活性显著降低,表明LPS应激造成机体抗氧化平衡失调,这与前人研究结果一致。
研究报道,饲粮中添加100、200和400 mg/kg PUE可提高肉鸡血清T-SOD活性和总抗氧化能力,降低血清MDA含量,缓解沙门氏菌感染引起的氧化应激[17]。臧佳佳等[18]研究表明,饲粮中添加20 mg/kg PUE可以降低大肠杆菌攻毒肉鸡血浆MDA和过氧化氢含量,并提高肠黏膜GSH-Px活性。Du等[16]研究报道,饲粮中添加200、400和800 mg/kg PUE可显著提高产蛋后期蛋鸡血清和肠道中抗氧化酶活性。本试验中,在应激条件下饲粮中添加PUE显著降低了肉仔鸡血清MDA含量,提高了血清抗氧化酶活性。综上所述,PUE可缓解机体氧化应激,可能是PUE通过调节核因子E2相关因子2(Nrf2)/血红素氧合酶-1(HO-1)抗氧化信号通路,提高抗氧化酶的基因表达和抗氧化酶活性,缓解LPS对机体和肠道的氧化损伤,进而改善免疫应激状态下肉仔鸡的生长性能[7,10]

3.3 PUE对LPS应激肉仔鸡血清免疫指标的影响

免疫球蛋白是体液免疫的重要组成部分,其含量在一定程度上反映了动物的免疫功能和生理状态[35]。有研究指出,低水平的免疫球蛋白表示机体免疫力降低,但高水平的免疫球蛋白表示机体可能处于炎症状态[36]。以往研究发现,LPS应激可引起肉鸡体液免疫应答,过度激活免疫系统,造成血清中免疫球蛋白含量显著提高[37]。本试验中,LPS应激极显著提高肉仔鸡血清IgA和IgG含量,这可能是肉鸡在LPS的作用下引起机体免疫应激反应,刺激浆细胞分泌大量的免疫球蛋白所导致的[38]。余应梅等[28]研究发现,饲粮中添加PUE可提高肉鸡血清IgA和IgG含量。本试验中,在非应激条件下,饲粮中添加PUE对肉仔鸡血清免疫球蛋白含量无显著影响;而在LPS应激条件下,饲粮中添加PUE显著降低了肉仔鸡血清IgA和IgG含量,表明PUE对应激状态下肉仔鸡的免疫功能具有调控作用。免疫球蛋白的合成需要动员机体大量的能量,这可能是LPS应激肉仔鸡生长性能降低,而饲粮中添加PUE改善了肉仔鸡生长性能的潜在原因[39]。但造成这一结果的具体原因有待进一步的研究。
LPS是革兰氏阴性菌细胞壁的主要成分,通过与细胞膜表面Toll样受体4(TLR4)结合,经髓样分化因子88(MyD88)依赖性或非依赖性途径,激活下游核转录因子-κB(NF-κB)炎症信号通路,引起TNF-α、IL-1β、IL-2和白细胞介素-6(IL-6)等促炎细胞因子的大量释放,造成机体炎症反应[40]。IL-10可抑制促炎细胞因子的产生,缓解机体过度的免疫反应[41]。Zhang等[42]研究发现,LPS应激显著提高肉鸡血清IL-1β、IL-6和TNF-α含量,并降低血清白细胞介素-4(IL-4)和IL-10含量,同时激活空肠和回肠中TLR4/NF-κB信号通路并上调IL-1βTNF-α的基因表达,引起机体过度炎症反应。本试验中,LPS应激使肉仔鸡血清IL-1β、IL-2和TNF-α含量显著升高,血清IL-10含量显著降低,说明LPS应激引起了机体炎症反应,造成促炎细胞因子的大量释放。PUE是一种天然植物多酚,具有较强的抗氧化和抗炎功能。研究发现,PUE在葡聚糖硫酸钠(DSS)诱导的结肠炎模型中可抑制NF-κB和促炎介质环氧化酶-2(COX-2)和诱导型一氧化氮合酶(iNOS)的表达,下调促炎细胞因子表达与分泌,缓解结肠炎症[7]。Zhou等[43]研究发现,饲粮中添加PUE可降低TNF-α的基因表达,并提高IL-10和TLR4/NF-κB信号通路中负调控因子的表达,抑制高迁移率族蛋白B1(HMGB1)/TLR4炎症信号通路,从而缓解氧化大豆油诱导的肉鸡肠道损伤。研究发现,PUE通过抑制Toll样受体6(TLR6)/MyD88/NF-κB信号通路,减少NF-κB核转位,下调促炎细胞因子分泌,缓解支原体感染引起的鸡胚肺部炎症损伤[44]。体外研究也发现,PUE通过调节NF-κB信号通路[45]、单磷酸腺苷活化蛋白激酶(AMPK)/沉默信息调节因子2相关酶1(SIRT1)信号通路[46]和脱铁性贫血相关的花生四烯酸等代谢途径[47],抑制促炎细胞因子的分泌,从而发挥抗炎作用。本试验中,在应激条件下饲粮中添加PUE显著降低了LPS应激肉仔鸡血清IL-1β和IL-2含量,这可能是PUE通过抑制NF-κB相关炎症信号通路,下调促炎细胞因子的表达,从而缓解机体炎症反应。

3.4 PUE对LPS应激肉仔鸡肠道通透性和黏膜形态的影响

D-LA和内毒素由肠道微生物代谢产生,正常情况下在血清中的含量较低,当肠道屏障受损和肠道通透性升高时,D-LA和内毒素会大量进入机体血液循环[48-49]。因此,血清中D-LA和内毒素的含量可作为衡量肠道通透性和肠道屏障完整性的指标[32]。研究发现,LPS应激会降低肉鸡肠道紧密连接蛋白表达,损伤肠道屏障,导致肠道通透性增加,引起血清D-LA含量显著升高[32,42]。本试验中,LPS应激使肉仔鸡血清D-LA和内毒素含量显著升高,说明LPS应激造成肠道屏障损伤并引起肠道通透性增加;而在应激条件下饲粮中添加PUE显著降低了血清内毒素含量,说明PUE对应激状态下肠道屏障完整性有一定的保护作用。
小肠是营养物质消化吸收的主要场所,其黏膜形态结构可以反映动物肠道健康和消化吸收能力。在一定范围内,较高的VH、较低的CD以及V/C的提高被认为具有更好的消化吸收能力[50]。研究表明,LPS应激会破坏肉鸡的肠道形态,降低VH和V/C,导致消化吸收能力和生长性能降低[32,51]。Li等[10]研究发现,PUE可促进空肠和回肠黏膜细胞增殖,提高紧密连接蛋白的基因表达,缓解敌草快诱导的肠道形态损伤。本试验中,LPS应激显著降低了肉仔鸡回肠VH和V/C,有降低十二指肠V/C和空肠VH的趋势,表明LPS应激造成肠道黏膜形态受损,这与前人的研究结果一致;在应激条件下饲粮中添加PUE显著提高了LPS应激肉仔鸡回肠VH,对回肠V/C也有一定程度的提高,说明PUE有助于改善应激状态下肉仔鸡的肠道形态,提高肠道对营养物质的消化吸收面积,从而改善生长性能。这可能是PUE通过提高肠道紧密连接蛋白的表达和增强杯状细胞的分泌功能,促进肠黏膜细胞增殖,恢复了肠道屏障完整性,从而缓解肠道形态损伤[7,10,52]

3.5 PUE对LPS应激肉仔鸡盲肠菌群的影响

家禽肠道内定植着多种不同种类的微生物菌群,菌群之间相互平衡,形成了相对稳定的微生态体系。肠道菌群将营养物质分解成短链脂肪酸(SCFA),可以为肠上皮细胞提供能量、拮抗病原微生物以及改善肠道屏障功能[53]。而肠道菌群失衡会损伤肠道屏障和肠道形态,诱发肠道炎症[54-55]。α多样性指数反映了微生物群落的丰富度和多样性。ACE指数和Chao1指数越高代表微生物群落的丰富度越高;Shannon指数越高代表微生物群落的多样性越高;Simpson指数越高代表微生物群落的多样性越低[56]。高水平的微生物多样性是肠道菌群成熟的标志,被认为有益于宿主健康,在应激条件下可以保持肠道微生态的稳定性[57]。本试验中,LPS应激有降低肉仔鸡盲肠菌群Shannon指数的趋势,表明LPS应激降低了盲肠微生物多样性并引起菌群结构的改变。
本研究中,肉仔鸡盲肠菌群在门水平上以厚壁菌门、拟杆菌门和变形菌门占比较大,为优势菌群。厚壁菌门和拟杆菌门下的许多菌种可以参与机体能量代谢,将复杂的碳水化合物和纤维素等营养物质分解,产生SCFA和维生素等益生物质,抑制有害菌的增殖,维持动物肠道健康[58];变形菌门中包括大量已知的病原有害菌(大肠杆菌、沙门氏菌和志贺氏菌等),其在机体发生代谢紊乱和肠道炎症时占比更高[59]。研究发现,LPS应激会降低肉鸡盲肠菌群中厚壁菌门相对丰度,并提高变形菌门相对丰度,造成肠道菌群紊乱[32,60]。本试验中,LPS应激有降低肉仔鸡盲肠厚壁菌门相对丰度的趋势,与前人研究结果基本一致。研究发现,饲粮中添加PUE可显著降低盲肠变形菌门相对丰度,缓解氧化大豆油引起的肉鸡菌群失调[15]。本试验中,饲粮中添加PUE对肉鸡盲肠菌群在门水平上的相对丰度未产生显著影响。动物肠道菌群受到环境、饮水、饲粮、动物品种和日龄等多因素的影响,造成上述结果差异的原因有待进一步论证。
本研究中,肉仔鸡盲肠菌群在属水平上以粪杆菌属、未定级梭菌纲UCG-014、乳杆菌属、瘤胃球菌属扭链群和未分类毛螺菌科占比较大,为主要优势菌属。Zhang等[32]研究发现,LPS应激显著提高了肉鸡盲肠变形菌门相对丰度,并降低了厚壁菌门和乳杆菌属相对丰度,引起肠道菌群失调并降低了盲肠SCFA含量。乳杆菌属是肠道有益菌,可产生SCFA并抑制大肠杆菌和沙门氏菌等有害菌的增殖,维持肠道屏障功能,对动物肠道健康有益[61]。UCG-005和norank_f_Eubacterium_coprostanoligenes_group归属于瘤胃球菌科,是重要的纤维降解菌,有利于动物对饲粮中纤维物质的消化与利用[62]。未定级梭菌纲vadinBB60群由条件致病菌组成,当肠道菌群失调时可能对机体产生负面影响[63-64]。埃希氏-志贺氏菌属是变形菌门中的一种肠道致病菌,其相对丰度的提高易引起肉鸡肠道菌群紊乱并引起生产性能降低[65]。丁酸球菌属是一种肠道有益菌,可产生丁酸盐发挥抗炎作用,保护肉鸡肠道健康[66]。本研究中,LPS应激极显著降低了肉仔鸡盲肠乳杆菌属和norank_f_Eubacterium_coprostanoligenes_group相对丰度,显著降低了盲肠未定级瘤胃球菌科相对丰度,有降低盲肠UCG-005相对丰度的趋势,显著提高了盲肠norank_f_norank_o_RF39和未定级梭菌纲vadinBB60群相对丰度,有提高盲肠埃希氏-志贺氏菌属相对丰度的趋势;饲粮中添加PUE极显著提高了盲肠丁酸球菌属相对丰度,有降低未定级梭菌纲vadinBB60群相对丰度的趋势。综上所述,LPS应激提高了有害菌的相对丰度,降低了微生物多样性以及SCFA产生菌和纤维降解菌的相对丰度,对肠道菌群产生了不利影响,可能会降低肉仔鸡对饲粮中纤维物质的消化与利用以及SCFA的产生,减少肠道对机体营养物质的供给,从而抑制动物的生长性能;在应激条件下饲粮中添加PUE可促进有益菌增殖,优化肠道菌群结构,这与PUE改善了LPS应激肉仔鸡生长性能的结论一致,说明良好的肠道菌群结构有利于维护肠道健康和提高营养物质的消化吸收,最终改善动物生长性能。

4 结论

综上所述,LPS应激对肉仔鸡的生长性能有负面影响,饲粮中添加750 mg/kg PUE可以缓解LPS应激造成的机体氧化应激和炎症反应,改善肠道形态和菌群结构,维护肠道健康,从而在一定程度上缓解了LPS应激对肉仔鸡的生长抑制和不利影响。
[1]
李嘉辉. 白藜芦醇对脂多糖刺激肉鸡生长性能、免疫功能和肠道屏障功能的影响[D]. 硕士学位论文. 保定: 河北农业大学,2022:12-13.

LI J H. Effects of resveratrol on growth performance,immune function and intestinal barrier function in broilers challenged with lipopolysaccharide[D]. Master’s Thesis. Baoding: Hebei Agricultural University,2022:12-13. (in Chinese)

[2]
DAI D, QI G H, WANG J, et al. Dietary organic acids ameliorate high stocking density stress-induced intestinal inflammation through the restoration of intestinal microbiota in broilers[J]. Journal of Animal Science and Biotechnology, 2022, 13(1):124.

DOI PMID

[3]
PHAM V H, ABBAS W, HUANG J, et al. Dietary coated essential oil and organic acid mixture supplementation improves health of broilers infected with avian pathogenic Escherichia coli[J]. Animal Nutrition, 2023,12:245-262.

[4]
LIU L L, GONG X Y, ZHANG X Y, et al. Resveratrol alleviates heat-stress-induced impairment of the jejunal mucosa through TLR4/MAPK signaling pathway in black-boned chicken[J]. Poultry Science, 2024, 103(1):103242.

[5]
孙永波, 王亚, 萨仁娜, 等. 家禽肠道健康评价指标研究进展[J]. 动物营养学报, 2017, 29(12):4266-4272.

SUN Y B, WANG Y, SA R N, et al. Research progress on evaluation indicators of intestinal health in poultry[J]. Chinese Journal of Animal Nutrition, 2017, 29(12):4266-4272. (in Chinese)

[6]
王晶, 许丽, 齐广海, 等. 家禽肠道健康及其营养调控措施[J]. 动物营养学报, 2019, 31(6):2479-2486.

WANG J, XU L, QI G H, et al. Intestinal health and its nutritional modulation measures of poultry[J]. Chinese Journal of Animal Nutrition, 2019, 31(6):2479-2486. (in Chinese)

[7]
JEON Y D, LEE J H, LEE Y M, et al. Puerarin inhibits inflammation and oxidative stress in dextran sulfate sodium-induced colitis mice model[J]. Biomedicine & Pharmacotherapy, 2020,124:109847.

[8]
PENG T, SHANG H L, YANG M R, et al. Puerarin improved growth performance and postmortem meat quality by regulating lipid metabolism of cattle under hot environment[J]. Animal Science Journal, 2021, 92(1):e13543.

[9]
王春花, 汪梦璐. 葛根素的生物学功能及其在畜禽生产中的应用[J]. 动物营养学报, 2022, 34(12):7489-7497.

DOI

WANG C H, WANG M L. Biological function of puerarin and its application of in livestock and poultry production[J]. Chinese Journal of Animal Nutrition, 2022, 34(12):7489-7497. (in Chinese)

DOI

[10]
LI M, YUAN D X, LIU Y H, et al. Dietary puerarin supplementation alleviates oxidative stress in the small intestines of diquat-challenged piglets[J]. Animals, 2020, 10(4):631.

[11]
WANG Q S, WANG Y L, ZHANG W Y, et al. Puerarin from Pueraria lobata alleviates the symptoms of irritable bowel syndrome-diarrhea[J]. Food & Function, 2021, 12(5):2211-2224.

[12]
WANG L, WU Y Z, ZHUANG L J, et al. Puerarin prevents high-fat diet-induced obesity by enriching Akkermansia muciniphila in the gut microbiota of mice[J]. PLoS One, 2019, 14(6):e0218490.

[13]
汪纪仓, 孙真真, 李思涵, 等. 葛根素对肉鸡生长性能、屠宰性能、肉品质、免疫器官指数及血清抗氧化指标的影响[J]. 黑龙江畜牧兽医, 2020(17):115-120.

WANG J C, SUN Z Z, LI S H, et al. Effects of puerarin on growth performance,slaughter performance,meat quality,immune organ index and serum antioxidant index of broilers[J]. Heilongjiang Animal Science and Veterinary Medicine, 2020(17):115-120. (in Chinese)

[14]
施璇. 葛根素对饲喂氧化大豆油黄羽肉鸡免疫器官结构和功能的影响[D]. 硕士学位论文. 南昌: 江西农业大学,2021:40-52.

SHI X. Effects of puerarin on the structure and function of immune organs in yellow feathered chickens fed with oxidized soybean oil[D]. Master’s Thesis. Nanchang: Jiangxi Agricultural University,2021:40-52. (in Chinese)

[15]
李君惠. 葛根素对饲喂氧化大豆油肉鸡盲肠抗氧化和屏障功能的影响[D]. 硕士学位论文. 南昌: 江西农业大学,2020:41-47.

LI J H. Effects of puerarin on antioxidant and barrier function of caecum in broilers fed oxidized soybean oil[D]. Master’s Thesis. Nanchang: Jiangxi Agricultural University,2020:41-47. (in Chinese)

[16]
DU X B, ZHAO D, PIAN H F, et al. Effects of puerarin as a feed additive on the laying performance,egg quality,endocrine hormones,antioxidant capacity,and intestinal morphology of aged laying hens[J]. Poultry Science, 2024, 103(5):103420.

[17]
LU Y, GUO X T, XU F G, et al. Protective effects of puerarin on liver tissue in Salmonella-infected chicks:a proteomic analysis[J]. Poultry Science, 2024, 103(1):103281.

[18]
臧佳佳, 李冰, 滕奕, 等. 葛根素对大肠杆菌感染肉鸡生长性能和肠道抗氧化功能及菌群的影响[J]. 中国畜牧兽医, 2023, 50(12):4846-4857.

DOI

ZANG J J, LI B, TENG Y, et al. Effect of puerarin on growth performance,intestinal antioxidant capacity and intestinal flora in broilers challenged with Escherichia coli[J]. China Animal Husbandry & Veterinary Medicine, 2023, 50(12):4846-4857. (in Chinese)

[19]
AN J S, SHI J J, LIU K B, et al. Effects of solid-state fermented wheat bran on growth performance,immune function,intestinal morphology and microflora in lipopolysaccharide-challenged broiler chickens[J]. Animals, 2022, 12(9):1100.

[20]
中华人民共和国农业农村部. 黄羽肉鸡营养需要量:NY/T 3645—2020[S]. 北京: 中国农业出版社, 2020.

Ministry of Agriculture and Rural Affairs of the People’s Republic of China. Nutrient requirements of yellow-feathered broilers:NY/T 3645—2020[S]. Beijing: China Agriculture Press, 2020. (in Chinese)

[21]
国家市场监督管理总局, 中国国家标准化管理委员会. 饲料中粗蛋白的测定凯氏定氮法:GB/T 6432—2018[S]. 北京: 中国标准出版社, 2018.

State Administration for Market Regulation, Standardization Administration of China. Determination of crude protein in feeds-Kjeldahl method:GB/T 6432—2018[S]. Beijing: Standards Press of China, 2018. (in Chinese)

[22]
国家市场监督管理总局, 中国国家标准化管理委员会. 饲料中钙的测定:GB/T 6436—2018[S]. 北京: 中国标准出版社, 2018.

State Administration for Market Regulation, Standardization Administration of China. Determination of calcium in feeds:GB/T 6436—2018[S]. Beijing: Standards Press of China, 2018. (in Chinese)

[23]
国家市场监督管理总局, 中国国家标准化管理委员会. 饲料中总磷的测定分光光度法:GB/T 6437—2018[S]. 北京: 中国标准出版社, 2018.

State Administration for Market Regulation, Standardization Administration of China. Determination of phosphorus in feeds-spectrophotometry:GB/T 6437—2018[S]. Beijing: Standards Press of China, 2018. (in Chinese)

[24]
熊本海, 罗清尧, 郑姗姗, 等. 中国饲料成分及营养价值表(2020年第31版)制订说明[J]. 中国饲料, 2020(21):87-97.

XIONG B H, LUO Q Y, ZHENG S S, et al. Tables of feed composition and nutritive in China(31th edition,2020)formulation description[J]. China Feed, 2020(21):87-97. (in Chinese)

[25]
叶金玲, 范秋丽, 林厦菁, 等. 牛樟芝多糖对脂多糖应激黄羽肉鸡生长性能和空肠黏膜完整性的影响[J]. 动物营养学报, 2021, 33(10):5601-5616.

DOI

YE J L, FAN Q L, LIN S J, et al. Effects of antredia cinnamomea polysaccharide on growth performance and jejunal mucosa integrity of yellow-feathered chickens challenged with lipopolysaccharide[J]. Chinese Journal of Animal Nutrition, 2021, 33(10):5601-5616. (in Chinese)

[26]
LI Y, ZHANG H, CHEN Y P, et al. Bacillus amyloliquefaciens supplementation alleviates immunological stress and intestinal damage in lipopolysaccharide-challenged broilers[J]. Animal Feed Science and Technology, 2015,208:119-131.

[27]
FAN Q L, ABOUELEZZ K F M, LI L, et al. Influence of mushroom polysaccharide,nano-copper,copper loaded chitosan,and lysozyme on intestinal barrier and immunity of LPS-mediated yellow-feathered chickens[J]. Animals, 2020, 10(4):594.

[28]
余应梅, 施璇, 王汝慧, 等. 葛根素对饲喂氧化大豆油黄羽肉鸡生长性能、抗氧化能力和免疫功能的影响[J]. 中国兽医学报, 2021, 41(7):1407-1413.

YU Y M, SHI X, WANG R H, et al. Effects of puerarin on growth performance,antioxidant capacity and immune function of yellow-feathered broilers fed with oxidized soybean oil[J]. Chinese Journal of Veterinary Science, 2021, 41(7):1407-1413. (in Chinese)

[29]
LU Y, GE S H, ZHANG H L, et al. Metabolomic and microbiome analysis of the protective effects of puerarin against Salmonella enteritidis infection in chicks[J]. BMC Veterinary Research, 2023, 19(1):242.

[30]
WANG Q Q, LIU T X, KOCI M, et al. Chlorogenic acid alleviated AFB1-induced hepatotoxicity by regulating mitochondrial function,activating Nrf2/HO-1,and inhibiting noncanonical NF-κB signaling pathway[J]. Antioxidants, 2023, 12(12):2027-2043.

[31]
WU S N, WANG L, CUI B L, et al. Effects of vitamin a on growth performance,antioxidants,gut inflammation,and microbes in weaned piglets[J]. Antioxidants, 2023, 12(12):2049.

[32]
ZHANG L H, WANG J, PIAO X S. Potential effects of 25-hydroxycholecalciferol on the growth performance,blood antioxidant capacity,intestinal barrier function and microbiota in broilers under lipopolysaccharide challenge[J]. Antioxidants, 2022, 11(11):2094.

[33]
SHU G, TANG Z T, DU H, et al. Effects of dietary ferulic acid supplementation on hepatic injuries in Tianfu broilers challenged with lipopolysaccharide[J]. Toxins, 2022, 14(3):227.

[34]
SUN L, XU G Q, DONG Y Y I, et al. Quercetin protects against lipopolysaccharide-induced intestinal oxidative stress in broiler chickens through activation of Nrf2 pathway[J]. Molecules, 2020, 25(5):1053.

[35]
GAO X L, GONG J A, YANG B W, et al. Effect of classical music on growth performance,stress level,antioxidant index,immune function and meat quality in broilers at different stocking densities[J]. Frontiers in Veterinary Science, 2023,10:1227654.

[36]
TAN T T, COUSSENS L M. Humoral immunity,inflammation and cancer[J]. Current Opinion in Immunology, 2007, 19(2):209-216.

[37]
杨敏敏, 车育彦, 王睿, 等. 枯草芽孢杆菌对脂多糖应激肉仔鸡生长性能、免疫性能和血清抗氧化性能的影响[J]. 动物营养学报, 2022, 34(4):2347-2360.

DOI

YANG M M, CHE Y Y, WANG R, et al. Effects of Bacillus subtilis on growth performance,immune performance and serum antioxidant performance of broilers challenged with lipopolysaccharide[J]. Chinese Journal of Animal Nutrition, 2022, 34(4):2347-2360. (in Chinese)

[38]
ZHANG P F, SHI B L, SU J L, et al. Relieving effect of Artemisia argyi aqueous extract on immune stress in broilers[J]. Journal of Animal Physiology and Animal Nutrition, 2017, 101(2):251-258.

[39]
康保聚. 血根碱对免疫应激断奶仔猪肠道黏膜损伤的修复作用研究[D]. 硕士学位论文. 长沙: 湖南农业大学, 2019.

KANG B J. A study on the repairing effect of sanguinarine on intestinal mucosal injury in immunological challenge weaned piglets[D]. Master’s Thesis. Changsha: Hunan Agricultural University, 2019. (in Chinese)

[40]
NIU Y, ZHAO Y W, HE J T, et al. Dietary dihydroartemisinin supplementation alleviates intestinal inflammatory injury through TLR4/NOD/NF-κB signaling pathway in weaned piglets with intrauterine growth retardation[J]. Animal Nutrition, 2021, 7(3):667-678.

DOI PMID

[41]
SABAT R, GRÜTZ G, WARSZAWSKA K, et al. Biology of interleukin-10[J]. Cytokine & Growth Factor Reviews, 2010, 21(5):331-344.

[42]
ZHANG R Q, LIU J S, LIU Y L, et al. Dietary garlic powder alleviates lipopolysaccharide-induced inflammatory response and oxidative stress through regulating the immunity and intestinal barrier function in broilers[J]. Animals, 2022, 12(17):2281.

[43]
ZHOU H, YU Y M, SHI X, et al. Dietary puerarin supplementation improves immune function in the small intestines of oxidized oil-challenged broilers[J]. Animal Science Journal, 2023, 94(1):e13895.

[44]
NIU L M, LUO R L, ZOU M Y, et al. Puerarin inhibits Mycoplasma gallisepticum (MG-HS)-induced inflammation and apoptosis via suppressing the TLR6/MyD88/NF-κB signal pathway in chicken[J]. International Immunopharmacology, 2020,88:106993.

[45]
HU W Z, YANG X J, ZHE C, et al. Puerarin inhibits iNOS, COX-2 and CRP expression via suppression of NF-κB activation in LPS-induced RAW264.7 macrophage cells[J]. Pharmacological Reports, 2011, 63(3):781-789.

PMID

[46]
PENG Z T, LIU H. Puerarin attenuates LPS-induced inflammatory injury in gastric epithelial cells by repressing NLRP3 inflammasome-mediated apoptosis[J]. Toxicology in Vitro, 2022,81:105350.

[47]
ZENG J Z, ZHAO N, YANG J J, et al. Puerarin induces molecular details of ferroptosis-associated anti-inflammatory on RAW264.7 macrophages[J]. Metabolites, 2022, 12(7):653.

[48]
YU J Y, ZHENG C B, ZHENG J, et al. Development of intestinal injury and restoration of weaned piglets under chronic immune stress[J]. Antioxidants, 2022, 11(11):2215.

[49]
LING Z, ZHANG L, ZHAN X A, et al. Effects of dietary supplementation of probiotic,Clostridium butyricum,on growth performance,immune response,intestinal barrier function,and digestive enzyme activity in broiler chickens challenged with Escherichia coli K88[J]. Journal of Animal Science and Biotechnology, 2016, 7(1):107-115.

[50]
YIN Y X, WANG F, YANG M, et al. Lycium barbarum polysaccharides as antibiotic substitutes improve growth performance,serum immunity,antioxidant status,and intestinal health for weaned piglets[J]. Frontiers in Microbiology, 2021,12:819993.

[51]
WEI Y, GAO Q Y, JING X Q, et al. Effect of cardamine violifolia on plasma biochemical parameters,anti-oxidative capacity,intestinal morphology,and meat quality of broilers challenged with lipopolysaccharide[J]. Animals, 2022, 12(19):2497.

[52]
LI J J, ZHANG L, LI Y F, et al. Puerarin improves intestinal barrier function through enhancing goblet cells and mucus barrier[J]. Journal of Functional Foods, 2020,75:104246.

[53]
XIA B, WU W D, ZHANG L, et al. Gut microbiota mediates the effects of inulin on enhancing sulfomucin production and mucosal barrier function in a pig model[J]. Food & Function, 2021, 12(21):10967-10982.

[54]
CHEN J M, WANG M C, ZHANG P, et al. Cordycepin alleviated metabolic inflammation in western diet-fed mice by targeting intestinal barrier integrity and intestinal flora[J]. Pharmacological Research, 2022,178:106191.

[55]
MA X, XU T T, QIAN M Q, et al. Faecal microbiota transplantation alleviates early-life antibiotic-induced gut microbiota dysbiosis and mucosa injuries in a neonatal piglet model[J]. Microbiological Research, 2021,255:126942.

[56]
张阳. 复合益生菌与黄芪多糖对生长育肥猪生长性能、免疫、 抗氧化及粪便微生物的影响[D]. 硕士学位论文. 成都: 四川农业大学, 2021.

ZHANG Y. Effects of compound probiotics and Astragalus polysaccharides on growth performance,immunity,antioxidation and fecal microbiota of growing-finishing pigs[D]. Master’s Thesis. Chengdu: Sichuan Agricultural University, 2021.in Chinese)

[57]
CHEN L M, XU Y S, CHEN X Y, et al. The maturing development of gut microbiota in commercial piglets during the weaning transition[J]. Frontiers in Microbiology, 2017,8:1688.

[58]
OAKLEY B B, LILLEHOJ H S, KOGUT M H, et al. The chicken gastrointestinal microbiome[J]. FEMS Microbiology Letters, 2014, 360(2):100-112.

DOI PMID

[59]
SHIN N R, WHON T W, BAE J W. Proteobacteria:microbial signature of dysbiosis in gut microbiota[J]. Trends in Biotechnology, 2015, 33(9):496-503.

[60]
YE J L, ZHANG C, FAN Q L, et al. Antrodia cinnamomea polysaccharide improves liver antioxidant,anti-inflammatory capacity,and cecal flora structure of slow-growing broiler breeds challenged with lipopolysaccharide[J]. Frontiers in Veterinary Science, 2022,9:994782.

[61]
XU Y T, LAHAYE L, HE Z X, et al. Micro-encapsulated essential oils and organic acids combination improves intestinal barrier function,inflammatory responses and microbiota of weaned piglets challenged with enterotoxigenic Escherichia coli F4 (K88+)[J]. Animal Nutrition, 2020, 6(3):269-277.

[62]
潘锋, 朱彦宾, 王之盛, 等. 酵母培养物和糖蜜对肉牛生长性能、营养物质表观消化率和粪便微生物区系组成的影响[J]. 动物营养学报, 2022, 34(2):1040-1049.

DOI

PAN F, ZHU Y B, WANG Z S, et al. Effects of yeast culture and molasses on growth performance,apparent digestibility of nutrients and fecal microflora composition of beef cattle[J]. Chinese Journal of Animal Nutrition, 2022, 34(2):1040-1049. (in Chinese)

[63]
XU S Y, JIAO C, DIAO Q Y, et al. Preweaning period is a critical window for rumen microbial regulation of average daily gain in Holstein heifer calves[J]. Journal of Animal Science and Biotechnology, 2023, 14(1):128.

DOI PMID

[64]
YAO Z T, LONG Y, YE J, et al. 16S rRNA Gene-based analysis reveals the effects of gestational diabetes on the gut microbiota of mice during pregnancy[J]. Indian Journal of Microbiology, 2020, 60(2):239-245.

DOI PMID

[65]
SOUZA M D, EECKHAUT V, GOOSSENS E, et al. Guar gum as galactomannan source induces dysbiosis and reduces performance in broiler chickens and dietary β-mannanase restores the gut homeostasis[J]. Poultry Science, 2023, 102(8):102810.

[66]
EECKHAUT V, WANG J, VAN PARYS A, et al. The probiotic butyricicoccus pullicaecorum reduces feed conversion and protects from potentially harmful intestinal microorganisms and necrotic enteritis in broilers[J]. Frontiers in Microbiology, 2016,7:1416.

文章导航

/