综述

柚皮素的生物学功能及其在畜禽生产中的应用

  • 王宜平 , 1 ,
  • 刘犇 , 1, 2, * ,
  • 郑文亚 1
展开
  • 1 宜春学院生命科学与资源环境学院,宜春 336000
  • 2 江西绿科农牧科技有限公司,宜春 336000
*刘 犇,副教授,E-mail:

王宜平(1993—),男,江西南昌人,助理实验师,硕士,从事反刍动物疾病防治研究。E-mail:

Copy editor: 田艳明

收稿日期: 2024-08-06

  网络出版日期: 2024-12-12

基金资助

江西省教育厅科技项目(GJJ201622)

江西省教育厅科技项目(GJJ211630)

江西省2023年“三区”人才支持计划项目

Biological Function of Naringenin and Its Application in Livestock and Poultry Production

  • WANG Yiping , 1 ,
  • LIU Ben , 1, 2, * ,
  • ZHENG Wenya 1
Expand
  • 1 College of Life Science and Resources and Environment, Yichun University, Yichun 336000, China
  • 2 Jiangxi Lvke Agriculture and Animal Husbandry Technology Co., Ltd., Yichun 336000, China
*associate professor, E-mail:

Received date: 2024-08-06

  Online published: 2024-12-12

摘要

柚皮素是一种天然的可生物降解黄酮类化合物,为柚皮苷的苷元,具有抗病原体、抗炎症、抗肿瘤、抗氧化、调节糖和脂代谢以及调节胃肠道功能等多种生物学功能,广泛应用于医药和食品等领域,可能成为天然绿色饲料添加剂和药物联合剂。本文从柚皮素的理化性质、生物学功能及其在畜禽生产中的应用进行综述,以期为柚皮素在畜禽生产中的开发和应用提供参考。

本文引用格式

王宜平 , 刘犇 , 郑文亚 . 柚皮素的生物学功能及其在畜禽生产中的应用[J]. 动物营养学报, 2024 , 36(12) : 7601 -7612 . DOI: 10.12418/CJAN2024.648

Abstract

Naringenin is a type of natural biodegradable flavonoid compound and serves as the aglycone of naringin. It exhibits a variety of biological functions, including anti-pathogenic, anti-inflammatory, anti-tumor, anti-oxidative, regulation of sugar and lipid metabolism, and regulation of gastrointestinal function. It is extensively utilized in medicine, food, and other domains and has the potential to become a natural green feed additive and drug combination agent. In this paper, the physicochemical properties, biological functions, and application of naringenin in livestock production are reviewed to provide a reference for the development and application of naringenin in livestock production.

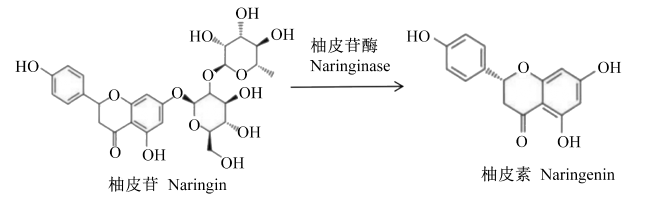
柚皮素(naringenin,NRG)存在于菝葜、化橘红、枳实和桃叶等天然植物中,同时作为一种自然界分布广泛的黄酮类化合物富含于水果、蔬菜和茶等日常饮食中,一般以柚皮苷的形式稳定存在于自然界中[1]。NRG是柚皮苷的苷元,柚皮苷摄入后被肠道细菌柚皮苷酶水解,产生2种中间体——鼠李糖和NRG(最活跃的糖苷配基形式),其中NRG更易于被胃肠道吸收,生物利用度高且安全剂量大[2];而且具有抗病原体、抗炎症、抗肿瘤、抗氧化、调节糖和脂代谢以及调节胃肠道功能等多种生物学功能,已广泛地应用于医药和食品等领域[3]。本文综述了NRG的理化性质、生物学功能以及其在畜牧生产中的应用研究进展,旨在为其在畜牧生产中的应用提供参考。

1 NRG的分布及其理化性质

NRG学名为4,5,7-三羟基二氢黄酮,化学式为C15H12O5,是一种二氢黄酮类化合物(化学结构见图1),存在于柑橘类水果中,被视为一种抗氧化剂和抗炎剂,可以通过血脑屏障[4]。NRG常温下为白色针状晶体,储存条件一般为阴凉干燥环境,相对分子质量为272.25,熔点为247~250 ℃。由于其分子内含有苯环、羟基和羰基等官能团,可溶于乙醇、乙醚和苯,但几乎不溶于水,脂溶性比水溶性好,科研工作者尝试通过给NRG连接脂溶性或水溶性较强的基团对其结构进行修饰或制成固体分散体、包合物和自微乳等各种剂型来提高其脂溶性或水溶性,从而提高其生物有效性[5],以期早日开发出可上市的新产品。
图1 柚皮苷和NRG的化学结构

Fig.1 Chemical structure of naringin and NRG

2 NRG的生物学功能及其机制

2.1 抗病原体

病原体与畜禽存在长期而复杂的斗争,病原体通过不断地繁殖、变异和进化来增强致病力和毒力,同时长期使用抗生素导致病原体的耐药性增强,急需寻找天然中草药类化合物进行治疗,NRG则发挥着重要作用。
对于细菌而言:研究发现NRG通过改变反异支链脂肪酸生物合成相关基因致使金黄色葡萄球菌膜通透性增加,使得蛋白质和核酸渗漏最终导致菌体死亡[6-7];Pawar等[8]研究发现,NRG抑制结核分枝杆菌-谷氨酸消旋酶活性,损伤细胞膜及细胞壁;此外,NRG降低了铜绿假单胞菌PAO1毒力因子控制基因(即lasllasRrhllrhlRlasAlasBphzA1和rhlA)的表达[9],抑制了鼠伤寒沙门氏菌的24个致病和17个鞭毛运动相关基因的表达,使得鼠伤寒沙门氏菌的毒力、代谢和转移下降[10];Yue等[11]研究发现,NRG下调变形链球菌gtfBgtfCcomDcomEluxS的mRNA表达,增加其表面疏水性,减少聚集,从而抑制细菌黏附和生物膜成熟;Andrade-Pavón等[12]研究发现,NRG通过抑制3-羟基-3-甲基戊二酰辅酶A还原酶(HMGR)和Ⅱ型DNA拓扑异构酶(TOPOⅡ)有效治疗念珠菌素引起的疾病;甚至,NRG可体内外与黏菌素产生协同作用[13]
对于病毒而言:NRG以剂量依赖性方式抑制白斑综合症病毒(WSSV)增殖,降低WSSV信号传导及转录激活蛋白(STAT)基因表达以阻止生命周期ie1基因的转录,显著提高WSSV攻击的小龙虾的存活率[14];NRG协同槲皮素、松属素抑制犬瘟热病毒核蛋白基因的表达[15],抑制细胞中高致病性禽流感H5N1毒株核蛋白的产生[16];此外,NRG与塞卡病毒NS2B-NS3蛋白酶结构域存在潜在相互作用,以浓度依赖性的方式阻止塞卡病毒复制和组装[17];NRG与鸡传染性喉气管炎(ILT)和传染性支气管炎(IB)2种病毒的外部包膜蛋白相互作用,抑制细胞外病毒[18];猪繁殖与呼吸综合综合征病毒(PRRSV)体外感染72 h后,NRG抑制细胞中病毒的复制[19]
对于寄生虫而言:NRG显著降低蜜蜂微孢子虫感染率,致使孢子数量减少量为64%,并且提高受感染蜜蜂存活率和蜂蜜产量[20-21];贾第鞭毛虫在NRG的治疗下,核膜及腹侧乳盘被损害,2 h丧失一半的种群[22];NRG通过激活核因子-κB(NF-κB)和诱导型一氧化氮合酶(iNOS)来增加一氧化氮(NO)和活性氧(ROS)含量,从而减少内脏利什曼原虫负荷,并使得前鞭毛体抑制在G0/G1期,使得宿主Th2免疫反应转换为Th1型[23];NRG抗艾美耳球虫功效达91.76%,减少了虫卵囊的排出量,降低了受感染羔羊的氧化应激,从而促进了羔羊平均日增重的提高[24]
综上可知,NRG可通过调控基因表达和抑制酶的作用来增加细菌的通透性,降低毒力和运动性;可通过抑制病毒生命周期基因和核蛋白基因的表达和包膜蛋白来抑制病毒的感染、复制和组装;还可抑制寄生虫的生长、虫卵囊的排出及降低感染畜禽氧化应激。这为NRG应用于预防畜禽感染病原体提供了可行性参考。

2.2 抗炎症

免疫反应是动物机体自身的防御机制,免疫机制削弱,病原微生物容易侵袭增殖感染;免疫机制增强,炎症则容易伤及到自身组织,因此,减轻炎症所带来的不必要的组织损伤是寻求的最佳结果。首先,NRG可通过抑制细胞表面Toll样受体2(TLR2)功能来抑制促炎细胞因子的产生并减弱NF-κB的激活[25]。核因子红细胞2相关因子2(Nrf2)是细胞内调节抗炎、抗凋亡和抗氧化基因表达的重要分子,可调控下游血红素氧化酶-1(HO-1)保护器官,NRG通过上调Nrf2/HO-1信号通路抑制百草枯诱导的炎症[26]。其次,NRG通过促进沉默信息调节因子1/叉头框蛋白O1(SIRT1/FOXO1)信号通路发挥抗炎作用,保护小鼠海马神经元HT22细胞免受氧糖剥夺/再灌注(OGD/R)诱导的细胞毒性,减弱OGD/R诱导的炎症反应[肿瘤坏死因子-α(TNF-α)、白细胞介素(IL)-1β、IL-6及IL-10水平降低][27]。再次,NRG可以减轻类风湿性关节炎大鼠的疼痛行为和关节指数评分,干扰线粒体裂变,从而抑制滑膜中CD4+ T细胞的极化和迁移,抑制促炎因子IL-6、TNF-α的基因表达,同时下降炎症和C反应蛋白(CRP)水平[28-29]。最后,NRG减轻狼疮临床表现的发展,抑制脾肿大并降低抗核和抗dsDNA自身抗体的水平,预防肾脏损伤并减少纤维化的发展,降低血清TNF-α、干扰素-γ(IFN-γ)和IL-6浓度[30]。NRG能够通过溶酶体和自噬防止脂多糖(LPS)诱导的肝损伤小鼠死亡并预防炎症诱导的器官损伤[31]。另外,NRG通过抗炎活性以及降低胞内磷脂酰肌醇3-激酶(PI3K)和蛋白激酶B(AKT)的总蛋白水平和磷酸化蛋白水平,显著提高LPS诱导的急性肺损伤小鼠的生存率,改善组织病理学变化,减轻肺水肿和肺血管渗漏,下调ROS水平,减少中性粒细胞浸润及血清和支气管肺泡灌洗液中炎症细胞因子的水平[32]。此外,NRG靶向巨噬细胞中10号染色体AKT级联的磷酸酶和张力蛋白同源物(PTEN),降低细胞外囊泡(EV)聚ADP核糖聚合酶(PARP)1的表达,下调EV miR21-3p,从而抑制巨噬细胞极化,维持香烟烟雾诱发的肺部疾病稳态[33]
综上所述,NRG可通过多途径、多靶点来发挥抗炎作用,其抗炎作用机制复杂,可调控TLR2/NF-κB、Nrf2/HO-1、SIRT1/FOXO1、PI3K/AKT及PTEN/AKT等信号通路,启动细胞内溶酶体和自噬,抑制CD4+ T细胞和巨噬细胞的极化来减轻机体炎症反应,避免组织损伤并减少纤维化。这提示NRG可应用于畜禽生产中,改善机体健康。

2.3 抗肿瘤

畜禽生产中家畜肿瘤性疾病研究较少,鸡马立克氏病(MD)、禽白血病(AL)和禽网状内皮组织增生症(RE)等家禽肿瘤病不仅直接影响了禽类的健康和生产性能,而且间接影响了动物产品和食品安全,造成了巨大经济损失,NRG则具备良好的抗肿瘤作用。
首先,NRG抑制氧化应激有效阻止化合物诱导的癌症发展:1)减轻脂质过氧化(增强自由基清除和抗氧化状态)和降低肝标志物酶水平[34];2)恢复还原型谷胱甘肽、氧化型谷胱甘肽、谷胱甘肽过氧化物酶(GPx)、谷胱甘肽还原酶(GR)和葡萄糖6-磷酸脱氢酶活性[35];3)恢复组织酶抗氧化剂[超氧化物歧化酶(SOD)、过氧化氢酶(CAT)、GPx、GR、谷胱甘肽S转移酶(GST)]和非酶抗氧化剂[谷胱甘肽(GSH)和维生素C]的活性[36];4)防止ROS的积累[37]。相反,NRG亦可促进氧化应激发挥抗肿瘤作用,激活ROS依赖性蛋白激酶——细胞外信号调节激酶(ERK)1/2诱导氧化应激和随后的胎盘绒毛膜癌细胞凋亡[38];激活ROS/凋亡信号调节激酶1(ASK1)信号通路导致氧化应激及胰腺癌细胞的凋亡[39]
其次,NRG减弱肿瘤细胞的活力和侵袭转移力:NRG激活前列腺癌细胞中AKT和ERK1/2信号通路靶向活力相关信号蛋白影响细胞活力[40]。此外,NRG可多途径抑制肿瘤侵袭、迁移和生长:1)调节肺癌细胞中环状叉头框蛋白M1(circFOXM1)/miR-3619-5p/精子相关抗原5(SPAG5)轴[41];2)抑制线粒体膜电位(MMP)、ERK和丝裂原活化蛋白激酶(MAPK)p38活性以及调节上皮间质转化(EMT)标志物[42];3)降低ERK1/2和c-Jun氨基末端激酶(JNK)/MAPK磷酸化,以剂量依赖性方式抑制恶性黑色素瘤中内皮细胞迁移、管形成和微血管萌芽[43];4)对SCN9A基因编码的电压门控钠通道具有直接或间接阻断活性抑制前列腺癌转移[44];5)抑制蛋白激酶C(PKC)活性来阻断转化生长因子-β1(TGF-β1)跨高尔基体网络的运输,导致乳腺癌细胞分泌TGF-β1减少,抑制转移[45]
再次,NRG可多位点致使癌细胞周期停滞:1)抑制细胞周期蛋白B1和细胞周期蛋白依赖性激酶1的表达并上调p21蛋白,诱导骨肉瘤细胞停滞在G2/M期[46];2)芹菜素和NRG的组合(CoAN)引起显著的细胞毒性,致使非小细胞肺癌细胞周期停滞在G2/M期[47];3)通过亚G1细胞群的积累、磷脂酰丝氨酸暴露、线粒体跨膜电位损失、DNA断裂、半胱天冬酶(Caspase)-3激活和Janus激酶(JAK)2/STAT3信号通路诱导肝癌细胞周期停滞和凋亡[48];4)抗氧化和抗炎作用将乳腺癌细胞发育阻滞在G0/G1期,以及阻滞亚G1期(75%)的细胞凋亡和沉积[49]
最后,NRG可多通路诱导肿瘤细胞凋亡和自噬:1)上调内质网应激信号通路标记物G蛋白偶联蛋白(GRP)78和GRP94介导凋亡,导致酸性囊泡细胞器形成并增加自噬溶酶体、微管相关蛋白轻链3-Ⅱ蛋白水平介导自噬[46];2)体内介导线粒体内在途径引起凋亡[49];3)上调B细胞淋巴瘤-2相关X蛋白(BAX)的表达,下调B细胞淋巴瘤-2(Bcl-2)的表达,增强Caspase-3/9活性,抑制IL-6在调节凋亡相关基因表达中的作用[50];4)显著上调Caspase-3和PARP蛋白的表达诱导细胞凋亡[43];5)槲皮素和NRG的组合(CoQN)可产生显著的细胞毒性,增强Caspase-3/7活性,增加脂质过氧化并降低MMP诱导的乳腺癌细胞凋亡[51];6)调节细胞增殖和凋亡相关基因[Bax、细胞周期蛋白D1(cyclin D1)、c-Myc、生存素(survivin)和Bcl-2]的表达以及PI3K/AKT通路的激活诱导甲状腺癌细胞凋亡[52];7)NRG和APO2配体(APO2L,也称为肿瘤坏死因子相关凋亡诱导配体)之间具有协同作用,NRG可恢复神经胶质瘤细胞对APO2L的敏感性,并通过激活Caspase,诱导p53、受体4和受体5的升高导致细胞凋亡[53]
此外,NRG具有协同临床药物和增强治疗性疫苗的抗肿瘤作用:1)通过提高ROS水平增强他莫昔芬对乳腺癌细胞的作用[54];2)联合紫杉醇增强对前列腺癌细胞的作用[40];3)联合环磷酰胺提高其抗肿瘤特性[50];4)使耐药肿瘤细胞组丝状伪足的长度和密度、集落形成、侵袭和伤口愈合均显著减少,增强对替莫唑胺耐药型癌的敏感性[55];5)促进树突状细胞的抗原提呈作用,诱导适度的细胞内氧化应激,导致溶酶体膜的破坏,增加抗原向胞浆的渗漏和交叉提呈[56]。这为家禽肿瘤病疫苗的设计提供了新思路。
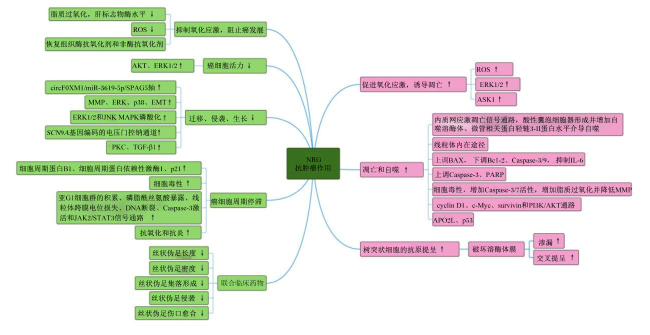
综上所述,NRG的抗肿瘤作用机制复杂(图2),其抑制氧化应激防止癌变的发展,或促进氧化应激致使癌细胞的凋亡;通过多种活性成分、多信号途径、多凋亡通路影响肿瘤细胞的生命周期、活力、侵袭力和迁移,同时可作为佐剂协同药物发挥抗肿瘤作用。目前,国内外关于NRG和畜禽肿瘤性疾病的相关研究几乎没有,其作用机制研究相对有限,该综述为后续的抗肿瘤和兽药疫苗的研究提供理论基础。
图2 NRG的抗癌作用机制

NRG:柚皮素 naringenin;ROS:活性氧 reactive oxygen species;AKT:蛋白激酶B protein kinase B;ERK:细胞外信号调节激酶 extracellular signal-regulated kinase;circFOXM1:环状叉头框蛋白M1 cyclic Forkhead box protein M1;SPAG5:精子相关抗原5 sperm-associated antigen 5;MMP:线粒体膜电位 mitochondrial membrane potential;EMT:上皮间质转化 epithelial-mesenchymal transition;JNK:c-Jun氨基末端激酶 c-Jun N-terminal kinase;MAPK:丝裂原活化蛋白激酶 mitogen activated protein kinase;PKC:蛋白激酶C protein kinase C;TGF-β1:转化生长因子-β1 transforming growth factor-β1;Caspase:半胱天冬酶 cysteinyl aspartate specific proteinase;JAK2:Janus激酶2 Janus kinase 2;STAT3:信号传导及转录激活蛋白3 signal transducer and activator of transcription 3;ASK1:凋亡信号调节激酶1 apoptotic signal-regulating kinase 1;BAX:B细胞淋巴瘤-2相关X蛋白 B-cell lymphoma-2 associated X protein;Bcl-2:B细胞淋巴瘤-2 B-cell lymphoma-2;IL-6:白细胞介素-6 interleukin-6;PARP:聚ADP核糖聚合酶 poly ADP-ribose polymerase;cyclin D1:细胞周期蛋白D1;survivin:生存素;PI3K:磷脂酰肌醇3-激酶 phosphatidylinositol 3-kinase;APO2L:APO2配体 APO2 ligand。

↑表示升高,↓表示降低。↑ indicated increase, and ↓ indicated decrease.

Fig.2 Anticancer mechanism of NRG

2.4 抗氧化

氧化应激是自由基在体内产生的一种负面影响,被认为是导致机体衰老和疾病的一个重要因素。研究发现,NRG可以通过恢复SODCATGSTGPx在内的抗氧化基因水平,提供抗氧化保护来最大限度地减少达沙替尼治疗白血病引起的肝毒性[57]。NRG通过Kelch样ECH关联蛋白1(Keap1)/Nrf2信号通路提高SOD、GPx和CAT活性[58]和调控PTEN/PI3K/AKT信号通路[59],抑制氧化应激来保护猪睾丸细胞。另有研究表明,NRG减弱了对甲基乙二醛处理的运动神经元样细胞中ROS的产生,并提高了GSH水平、SOD活性和Nrf2核表达;然而胰岛素样生长因子-1受体(IGF-1R)拮抗剂AG1024减弱了该抗氧化作用;因此,IGF-1R途径介导的抗氧化防御在NRG保护机制中发挥着重要作用[60]。另有研究发现,NRG可以调节受体相互作用蛋白(RIP)1、RIP3-混合谱系激酶结构域(MLKL)信号通路来减轻球囊损伤诱导的氧化应激,从而抑制球囊损伤诱导的血管新生内膜增生[61]。此外,NRG抗氧化作用保护小鼠免受乙醇诱导的出血性损伤、上皮细胞损失和白细胞水肿,通过抑制NF-κB活性和降低NO、丙二醛(MDA)、TNF-α和髓过氧化物酶(MPO)水平来减轻胃溃疡;同时,抑制NF-κB和MAPK信号通路,抑制胃上皮细胞分泌TNF-α、IL-6和IL-8,以及环氧合酶-2(COX-2)和iNOS[62]。综上所述,NRG通过直接清除自由基、调节抗氧化酶系统和参与氧化还原体系等途径发挥较强的抗氧化作用。

2.5 调节糖和脂代谢

随着社会经济的发展和主人的过度溺爱,动物肥胖问题在世界范围内急剧增加。它会显著增加动物患代谢紊乱、内分泌失调、心肺疾病、关节疾病、生长发育异常和繁殖障碍等疾病的风险,亟待引起重视[63]。NRG具有较强的促脂质和糖类代谢能力。研究发现,NRG在无肥胖或高脂肪饮食的情况下可保持有效的代谢特性,增强肝脏脂肪酸氧化,降低血浆脂质并增强胰岛素敏感性;此外,NRG增加了小鼠在黑暗周期中的呼吸交换率和食物消耗[64]。NRG在高脂饮食诱导的肥胖进展阶段仍具有调控肥胖降血脂和血糖功能。其一,NRG通过降低胆固醇、甘油三酯和低密度脂蛋白(LDL)含量、并提高高密度脂蛋白(HDL)含量来调节脂质紊乱;通过调节脂肪细胞因子并降低STAT3的磷酸化,降低血清MDA和NO含量,并提高血清SOD活性和GSH含量等氧化应激因子水平改善肥胖[65]。其二,NRG通过抑制JNK途径抑制单核细胞趋化蛋白(MCP)表达来抑制巨噬细胞和中性粒细胞浸润脂肪组织[66-67],通过减轻促炎因子TNF-α和IL-6分泌,预防糖尿病和动脉粥样硬化等脂肪组织慢性炎症[68]。其三,NRG可减少细胞中的脂质积累,增加葡萄糖摄取,降低ATP含量,激活钙离子/钙调素依赖蛋白激酶激酶β(CaMKKβ)/单磷酸腺苷活化蛋白激酶(AMPK)/乙酰辅酶A羧化酶(ACC)信号通路,并增强脂肪细胞和成肌细胞肌管中的线粒体生物合成,促进脂肪细胞和成肌细胞自噬流的启动[69]。其四,NRG可能通过限制前脂肪细胞的分化,显著诱导胰岛素来抵抗和降低成熟脂肪细胞中脂联素的表达[70]
另有研究表明,NRG通过增加PI3K和ERK1/2的磷酸化来刺激低密度脂蛋白胆固醇(LDL-C)基因的表达,从而增强肝癌细胞中转录因子、甾醇调节元件结合蛋白(SREBP)水平并促进其蛋白成熟,有效降低动脉粥样硬化和冠心病的死亡率和发病率[71]。NRG可减轻雌性小鼠卵巢切除相关的许多代谢紊乱。在卵巢切除小鼠中,NRG使其表现出较低的空腹血糖和胰岛素水平,腹内和皮下脂肪减少50%以上,血浆瘦素和脂肪库中的瘦素mRNA降低,肝脏脂质积累减少,并且与脂肪生成、脂肪酸氧化和糖异生相关的肝脏基因表达也发生相应改变[72]
由此可见,NRG通过调节脂质代谢、葡萄糖代谢和代谢综合征的炎症来发挥降血脂和抗血糖功能。摄入NRG对动物肥胖相关疾病(高脂血症、胰岛素抵抗、动脉粥样硬化和冠心病等)具有良好预防和治疗效用。

2.6 调节胃肠道功能

近年来,NRG与肠道相互作用的研究引发了食品科学、营养学和生物医学等领域的广泛关注。维持肠道稳态对畜禽健康起着至关重要的作用,一旦肠道失调,则可能引发多种疾病[73]。NRG可改善肠道屏障,调节通透性以维持肠道稳态。研究发现,NRG通过显著减少产肠毒素大肠杆菌(ETEC)感染仔猪空肠黏膜炎性介质的含量,提高肠道绒毛高度和绒毛高度与隐窝深度的比值来改善肠道屏障[74]。NRG通过抑制NF-κB介导的肌球蛋白轻链激酶(MLCK)/磷酸化肌球蛋白轻链(p-MLC)和NOD样受体pyrin结构域相关蛋白3(NLRP3)信号通路来维持紧密连接蛋白模式,明显减轻TNF-α诱导的体外肠血管屏障破坏[75]。NRG显著减少固有层辅助性T细胞17(Th17)数量,维持结肠长度来增强肠道通透性,以抑制结肠炎的发展[76]。此外,NRG为黄酮类化合物代谢产物之一,普遍存在于蔬菜和水果中,是丰富的抗氧化剂,可影响肠道菌群代谢和生物转化[77]。NRG通过调节肠道菌群的生长、组成、结构和基因表达变化来调节肠道微生物菌群[78]。NRG线性提高粪便中总挥发性脂肪酸、乙酸盐和丁酸盐的含量,影响肠道菌群相对丰度(表1),但不影响肠道微生物多样性和群落结构[79]。综上所述,在维持动物机体肠道稳态中,NRG发挥较强的改善作用,其作用途径主要包括:1)保护肠道屏障调节通透性;2)影响免疫系统;3)影响肠道菌群代谢;4)调节肠道菌群的丰富度。
表1 NRG对肠道菌群的影响

Table 1 Effects of NRG on intestinal microbiota

项目
Item
影响作用
Effects
肠道菌群
Intestinal microbiota
柚皮素
Naringenin
提高丰度 双歧杆菌属(Bifidobacterium)、丁酸梭菌属(Butyrivibrio)、
球形梭菌-直肠真杆菌群(Clostridium coccoides-Eubacterium rectale group)、
普拉梭菌(Faecalibacterium prausnitzii)、普雷沃氏菌属(Prevotella)、
柏林密螺旋体菌(Treponema berlinense)
降低丰度 嗜胆菌属(Bilophila)、肠球菌属(Enterococcus)、乳梭菌属
(Lachnoclostridium)、毛螺菌属(Lachnospira)、
甲烷八叠球菌属(Methanosarcina)、罗氏菌属(Roseburia)、瘤胃球菌
属扭链群(Ruminococcus_torques_group)

3 NRG对畜禽抗氧化和免疫功能的影响

在天然植物提取物对畜禽生产的应用研究中,植物提取物已显示出对畜禽生产性能、生长性能、抗氧化能力和肠道免疫力的有益作用。研究发现,NRG通过调节凋亡基因的表达来改善解冻后公鸡精液的质量和生育能力[80]。精液保存液添加25 μmol/L NRG可为储存的猪精液提供显著的膜稳定化作用,也为防止脂质过氧化和减少ROS生成量等发挥保护作用[81]。由此可见,NRG具备开发为畜禽精液保护液添加剂的潜力。Lien等[82]研究发现,NRG显著降低鸡蛋蛋黄中胆固醇含量,增加蛋重及蛋黄重/蛋重比例,升高血清SOD活性,降低血清胆固醇和甘油三酯含量,同时总抗氧化能力、硫代巴比妥酸反应物水平和超氧化物清除能力高于对照组。Poapolathep等[83]研究表明,连续3 d口服25 mg/kg NRG有效增加静脉注射呕吐毒素仔猪的毒素排泄,减少氧化应激,减少呕吐毒素对仔猪的损害。Wang等[74]报道,饲粮中添加50~200 mg/kg番石榴叶提取物可降低仔猪腹泻发生率,提高血清SOD、GSH-Px活性和总抗氧化能力,降低仔猪血清和空肠黏膜中促炎细胞因子,提高仔猪空肠绒毛高度和绒毛高度与隐窝深度的比值。Niu等[84]研究发现,NRG显著降低促炎细胞因子IL-8含量,提高仔猪肠道总抗氧化能力和SOD活性,同时增加仔猪结肠微生物群落的α多样性。以上试验结果归因于NRG的抗氧化和抗炎能力。奶牛体细胞数是衡量奶牛生理健康状况的重要指标,直接指证奶牛乳腺炎疾病。研究表明,在患有乳腺炎的奶牛乳房内给药30 mg/d NRG可改善奶牛乳腺炎[85]。此外,饲喂黄酮提取物具有调节泌乳奶牛的胃肠微生物组和新陈代谢的作用,从而降低奶牛的全身内毒素水平[79]和恢复奶牛泌乳性能[86]。给自然感染艾美耳球虫的羔羊连续90 d每天饲喂5 mg/kg NRG,抗球虫功效达91.76%,显著减少球虫卵囊的产量并促进受感染羔羊的日增重[24]。由此可见,NRG及其黄酮类化合物能有效改善畜禽肠道微生物组,维护肠道屏障,提高抗炎和抗氧化能力,改善畜禽生产性能,显示出NRG作为畜禽饲粮添加剂和精液保护液添加剂的潜力,但目前单一的NRG在畜禽生产的应用效果研究较少。

4 小结

在抗生素、常规药物以及疫苗保护力下降的背景下,NRG作为天然植物菝葜、化橘红、枳实和桃叶的主要成分,存在于水果、蔬菜和茶等日常饮食中,不仅具有多种生物学功能,而且可提高畜禽的生产性能、繁殖性能、抗炎能力和改善肠道微生物群落,具有较好的应用前景。但目前关于NRG在畜禽生产中的研究相对较少,不能明确同品种不同生长阶段或不同品种畜禽的最适添加剂量及作用效果。因此,未来应加强天然化合物NRG在畜禽生产上的研究,为饲料禁抗背景下NRG在畜禽生产上的开发和应用提供依据。
[1]
唐镜, 谭若兰, 吕中建, 等. 柚皮素的提取及其抗癌作用研究进展[J]. 绿色科技, 2019(8):240-244.

TANG J, TAN R L, LV Z J, et al. Research progress on extraction of naringenin and its anti-cancer activity[J]. Journal of Green Science and Technology, 2019(8):240-244. (in Chinese)

[2]
曾文峰, 张发云, 杜刚军, 等. 柚皮素:新一代免疫调节剂[J]. 生物化学与生物物理进展, 2018, 45(9):915-925.

ZENG W F, ZHANG F Y, DU G J, et al. Research updates on a novel immunomodulator,naringenin[J]. Progress in Biochemistry and Biophysics, 2018, 45(9):915-925. (in Chinese)

[3]
ARAFAH A, REHMAN M U, MIR T M, et al. Multi-therapeutic potential of naringenin (4',5,7-trihydroxyflavonone):experimental evidence and mechanisms[J]. Plants (Basel,Switzerland), 2020, 9(12):1784.

[4]
王凯华, 李配庆, 陈真珍. 柚皮素神经保护作用的研究进展[J]. 中国实用神经疾病杂志, 2020, 23(4):358-362.

WANG K H, LI P Q, CHEN Z Z. Research progress on naringenin’s neuroprotective effect[J]. Chinese Journal of Practical Nervous Diseases, 2020, 23(4):358-362. (in Chinese)

[5]
季鹏, 赵文明, 于桐. 柚皮素的最新研究进展[J]. 中国新药杂志, 2015, 24(12):1382-1386, 1392.

JI P, ZHAO W M, YU T. Recent research progress of naringenin[J]. Chinese Journal of New Drugs, 2015, 24(12):1382-1386, 1392. (in Chinese)

[6]
GAO Y, JI Y B, LI W L, et al. Endophytic fungi from Dalbergia odorifera T.Chen producing naringenin inhibit the growth of Staphylococcus aureus by interfering with cell membrane,DNA,and protein[J]. Journal of Medicinal Food, 2021, 24(2):116-123.

[7]
WANG L H, ZENG X A, WANG M S, et al. Modification of membrane properties and fatty acids biosynthesis-related genes in Escherichia coli and Staphylococcus aureus:implications for the antibacterial mechanism of naringenin[J]. Biochimica et Biophysica Acta:Biomembranes, 2018, 1860(2):481-490.

[8]
PAWAR A, JHA P, CHOPRA M, et al. Screening of natural compounds that targets glutamate racemase of Mycobacterium tuberculosis reveals the anti-tubercular potential of flavonoids[J]. Scientific Reports, 2020, 10(1):949.

[9]
VANDEPUTTE O M, KIENDREBEOGO M, RASAMIRAVAKA T, et al. The flavanone naringenin reduces the production of quorum sensing-controlled virulence factors in Pseudomonas aeruginosa PAO1[J]. Microbiology (Reading,England), 2011, 157(Pt 7):2120-2132.

[10]
VIKRAM A, JESUDHASAN P R, JAYAPRAKASHA G K, et al. Citrus flavonoid represses Salmonella pathogenicity island 1 and motility in S. typhimurium LT2[J]. International Journal of Food Microbiology, 2011, 145(1):28-36.

[11]
YUE J X, YANG H Y, LIU S Y, et al. Influence of naringenin on the biofilm formation of Streptococcus mutans[J]. Journal of Dentistry, 2018, 76:24-31.

[12]
ANDRADE-PAVÓN D, GÓMEZ-GARCÍA O, VILLA-TANACA L. Molecular recognition of citroflavonoids naringin and naringenin at the active site of the HMG-CoA reductase and DNA topoisomerase type Ⅱ enzymes of Candida spp. and Ustilago maydis[J]. Indian Journal of Microbiology, 2022, 62(1):79-87.

[13]
XU M X, YAO Z C, ZHAO Y N, et al. Naringenin restores colistin activation against colistin-resistant gram-negative bacteria in vitro and in vivo[J]. Frontiers in Microbiology, 2022, 13:916587.

[14]
SUN Z C, CHEN C, XU F F, et al. Evaluation of the antiviral activity of naringenin,a major constituent of Typha angustifolia,against white spot syndrome virus in crayfish Procambarus clarkii[J]. Journal of Fish Diseases, 2021, 44(10):1503-1513.

[15]
GONZÁLEZ-BÚRQUEZ M D J, GONZÁLEZ-DÍAZ F R, GARCÍA-TOVAR C G, et al. Comparison between in vitro antiviral effect of Mexican propolis and three commercial flavonoids against canine distemper virus[J]. Evidence-Based Complementary and Alternative Medicine:eCAM, 2018, 2018:7092416.

[16]
SITHISARN P, MICHAELIS M, SCHUBERT-ZSILAVECZ M, et al. Differential antiviral and anti-inflammatory mechanisms of the flavonoids biochanin A and baicalein in H5N1 influenza A virus-infected cells[J]. Antiviral Research, 2013, 97(1):41-48.

DOI PMID

[17]
CATANEO A H D, KUCZERA D, KOISHI A C, et al. The citrus flavonoid naringenin impairs the in vitro infection of human cells by Zika virus[J]. Scientific Reports, 2019, 9(1):16348.

[18]
ABO-EL-YAZID Z H, AHMED O K, EL-THOLOTH M, et al. Green synthesized silver nanoparticles using Cyperus rotundus L. extract as a potential antiviral agent against infectious laryngotracheitis and infectious bronchitis viruses in chickens[J]. Chemical and Biological Technologies in Agriculture, 2022, 9:55.

[19]
ARJIN C, HONGSIBSONG S, PRINGPROA K, et al. Effect of ethanolic Caesalpinia sappan fraction on in vitro antiviral activity against porcine reproductive and respiratory syndrome virus[J]. Veterinary Sciences, 2021, 8(6):106.

[20]
KLASSEN S S, VANBLYDERVEEN W, ECCLES L, et al. Nosema ceranae infections in honey bees (Apis mellifera) treated with pre/probiotics and impacts on colonies in the field[J]. Veterinary Sciences, 2021, 8(6):107.

[21]
BORGES D, GUZMAN-NOVOA E, GOODWIN P H. Control of the microsporidian parasite Nosema ceranae in honey bees (Apis mellifera) using nutraceutical and immuno-stimulatory compounds[J]. PLoS One, 2020, 15(1):e0227484.

[22]
RUFINO-GONZÁLEZ Y, PONCE-MACOTELA M, GONZÁLEZ-MACIEL A, et al. In vitro activity of the F-6 fraction of oregano against Giardia intestinalis[J]. Parasitology, 2012, 139(4):434-440.

[23]
KAUR G, CHAUHAN K, KAUR S. Immunotherapeutic potential of Codonopsis clematidea and naringenin against visceral leishmaniasis[J]. Biomedicine & Pharmacotherapy, 2018, 108:1048-1061.

[24]
PÉREZ-FONSECA A, ALCALA-CANTO Y, SALEM A Z M, et al. Anticoccidial efficacy of naringenin and a grapefruit peel extract in growing lambs naturally-infected with Eimeria spp.[J]. Veterinary Parasitology, 2016, 232:58-65.

[25]
KATAOKA H, SAEKI A, HASEBE A, et al. Naringenin suppresses Toll-like receptor 2-mediated inflammatory responses through inhibition of receptor clustering on lipid rafts[J]. Food Science & Nutrition, 2021, 9(2):963-972.

[26]
DE OLIVEIRA M R, ANDRADE C M B, FÜRSTENAU C R. Naringenin exerts anti-inflammatory effects in paraquat-treated SH-SY5Y cells through a mechanism associated with the Nrf2/HO-1 axis[J]. Neurochemical Research, 2018, 43(4):894-903.

DOI PMID

[27]
ZHAO P, LU Y, WANG Z Y. Naringenin attenuates cerebral ischemia/reperfusion injury by inhibiting oxidative stress and inflammatory response via the activation of SIRT1/FOXO1 signaling pathway in vitro[J]. Acta Cirurgica Brasileira/Sociedade Brasileira Para Desenvolvimento Pesquisa em Cirurgia, 2023, 38:e380823.

[28]
HAJIZADEH A, ABTAHI FROUSHANI S M, TEHRANI A A, et al. Effects of naringenin on experimentally induced rheumatoid arthritis in Wistar rats[J]. Archives of Razi Institute, 2021, 76(4):903-912.

[29]
JIANG Y P, WEN J J, ZHAO X X, et al. The flavonoid naringenin alleviates collagen-induced arthritis through curbing the migration and polarization of CD4+ T lymphocyte driven by regulating mitochondrial fission[J]. International Journal of Molecular Sciences, 2022, 24(1):279.

[30]
ABREGO-PEREDO A, ROMERO-RAMÍREZ H, ESPINOSA E, et al. Naringenin mitigates autoimmune features in lupus-prone mice by modulation of T-cell subsets and cytokines profile[J]. PLoS One, 2020, 15(5):e0233138.

[31]
JIN L T, ZENG W F, ZHANG F Y, et al. Naringenin ameliorates acute inflammation by regulating intracellular cytokine degradation[J]. Journal of Immunology (Baltimore,Md.:1950), 2017, 199(10):3466-3477.

[32]
ZHAO M H, LI C, SHEN F J, et al. Naringenin ameliorates LPS-induced acute lung injury through its anti-oxidative and anti-inflammatory activity and by inhibition of the PI3K/AKT pathway[J]. Experimental and Therapeutic Medicine, 2017, 14(3):2228-2234.

DOI PMID

[33]
CHEN Z, WU H, FAN W Y, et al. Naringenin suppresses BEAS-2B-derived extracellular vesicular cargoes disorder caused by cigarette smoke extract thereby inhibiting M1 macrophage polarization[J]. Frontiers in Immunology, 2022, 13:930476.

[34]
ARUL D, SUBRAMANIAN P. Inhibitory effect of naringenin (citrus flavonone) on N-nitrosodiethylamine induced hepatocarcinogenesis in rats[J]. Biochemical and Biophysical Research Communications, 2013, 434(2):203-209.

DOI PMID

[35]
GANAPATHY E, PERAMAIYAN R, RAJASEKARAN D, et al. Modulatory effect of naringenin on N-methyl-N'-nitro-N-nitrosoguanidine- and saturated sodium chloride-induced gastric carcinogenesis in male Wistar rats[J]. Clinical and Experimental Pharmacology & Physiology, 2008, 35(10):1190-1196.

[36]
BODDULURU L N, KASALA E R, MADHANA R M, et al. Naringenin ameliorates inflammation and cell proliferation in benzo (a) pyrene induced pulmonary carcinogenesis by modulating CYP1A1,NFκB and PCNA expression[J]. International Immunopharmacology, 2016, 30:102-110.

[37]
ZHANG L R, XU X H, JIANG T C, et al. Citrus aurantium naringenin prevents osteosarcoma progression and recurrence in the patients who underwent osteosarcoma surgery by improving antioxidant capability[J]. Oxidative Medicine and Cellular Longevity, 2018, 2018:8713263.

[38]
PARK S, LIM W, BAZER F W, et al. Naringenin suppresses growth of human placental choriocarcinoma via reactive oxygen species-mediated P38 and JNK MAPK pathways[J]. Phytomedicine, 2018, 50:238-246.

DOI PMID

[39]
PARK H J, CHOI Y J, LEE J H, et al. Naringenin causes ASK1-induced apoptosis via reactive oxygen species in human pancreatic cancer cells[J]. Food and Chemical Toxicology:an International Journal Published for the British Industrial Biological Research Association, 2017, 99:1-8.

[40]
LIM W, PARK S, BAZER F W, et al. Naringenin-induced apoptotic cell death in prostate cancer cells is mediated via the PI3K/AKT and MAPK signaling pathways[J]. Journal of Cellular Biochemistry, 2017, 118(5):1118-1131.

DOI PMID

[41]
TAN Z F, SUN Y L, LIU M, et al. Retracted:naringenin inhibits cell migration,invasion,and tumor growth by regulating circFOXM1/miR-3619-5p/SPAG5 axis in lung cancer[J]. Cancer Biotherapy and Radiopharmaceuticals, 2020, 35(10):e826-e838.

[42]
CHEN Y Y, CHANG Y M, WANG K Y, et al. Naringenin inhibited migration and invasion of glioblastoma cells through multiple mechanisms[J]. Environmental Toxicology, 2019, 34(3):233-239.

[43]
CHOI J, LEE D H, JANG H, et al. Naringenin exerts anticancer effects by inducing tumor cell death and inhibiting angiogenesis in malignant melanoma[J]. International Journal of Medical Sciences, 2020, 17(18):3049-3057.

DOI PMID

[44]
AKTAS H G, AKGUN T. Naringenin inhibits prostate cancer metastasis by blocking voltage-gated sodium channels[J]. Biomedicine & Pharmacotherapy, 2018, 106:770-775.

[45]
ZHANG F Y, DONG W J, ZENG W F, et al. Naringenin prevents TGF-β1 secretion from breast cancer and suppresses pulmonary metastasis by inhibiting PKC activation[J]. Breast Cancer Research, 2016, 18(1):38.

DOI PMID

[46]
LEE C W, HUANG C C Y, CHI M C, et al. Naringenin induces ROS-mediated ER stress,autophagy,and apoptosis in human osteosarcoma cell lines[J]. Molecules, 2022, 27(2):373.

[47]
LIU X X, ZHAO T, SHI Z, et al. Synergism antiproliferative effects of apigenin and naringenin in NSCLC cells[J]. Molecules, 2023, 28(13):4947.

[48]
ZHANG M, LAI J M, WU Q L, et al. Naringenin induces HepG2 cell apoptosis via ROS-mediated JAK-2/STAT-3 signaling pathways[J]. Molecules, 2023, 28(11):4506.

[49]
ZHAO Z J, JIN G G, GE Y H, et al. Naringenin inhibits migration of breast cancer cells via inflammatory and apoptosis cell signaling pathways[J]. Inflammopharmacology, 2019, 27(5):1021-1036.

DOI PMID

[50]
NOORI S, REZAEI TAVIRANI M, DERAVI N, et al. Naringenin enhances the anti-cancer effect of cyclophosphamide against MDA-MB-231 breast cancer cells via targeting the STAT3 signaling pathway[J]. Iranian Journal of Pharmaceutical Research:IJPR, 2020, 19(3):122-133.

[51]
RHMAN M A, DEVNARAIN N, KHAN R, et al. Synergism potentiates oxidative antiproliferative effects of naringenin and quercetin in MCF-7 breast cancer cells[J]. Nutrients, 2022, 14(16):3437.

[52]
ZHOU J, XIA L, ZHANG Y. Naringin inhibits thyroid cancer cell proliferation and induces cell apoptosis through repressing PI3K/AKT pathway[J]. Pathology,Research and Practice, 2019, 215(12):152707.

[53]
SONG T, ZHANG M Y, WU J, et al. Glioma progression is suppressed by naringenin and APO2L combination therapy via the activation of apoptosis in vitro and in vivo[J]. Investigational New Drugs, 2020, 38(6):1743-1754.

[54]
XU Z X, HUANG B, LIU J, et al. Combinatorial anti-proliferative effects of tamoxifen and naringenin:the role of four estrogen receptor subtypes[J]. Toxicology, 2018, 410:231-246.

[55]
JAYALAKSHMI J, VANISREE A J. Naringenin sensitizes resistant C6 glioma cells with a repressive impact on the migrating ability[J]. Annals of Neurosciences, 2020, 27(3/4):114-123.

[56]
WANG L Y, ZENG W F, WANG L Y, et al. Naringenin enhances the antitumor effect of therapeutic vaccines by promoting antigen cross-presentation[J]. Journal of Immunology (Baltimore,Md.:1950), 2020, 204(3):622-631.

[57]
ALANAZI A Z, ALHAZZANI K, ALREWILY S Q, et al. The potential protective role of naringenin against dasatinib-induced hepatotoxicity[J]. Pharmaceuticals (Basel,Switzerland), 2023, 16(7):921.

[58]
CHEN H J, CHEN J Q, SHI X, et al. Naringenin protects swine testis cells from bisphenol A-induced apoptosis via Keap1/Nrf2 signaling pathway[J]. BioFactors, 2022, 48(1):190-203.

[59]
CHEN H J, ZHANG Y, ZOU M M, et al. Dibutyl phthalate-induced oxidative stress and apoptosis in swine testis cells and therapy of naringenin via PTEN/PI3K/AKT signaling pathway[J]. Environmental Toxicology, 2022, 37(8):1840-1852.

DOI PMID

[60]
TSENG Y T, HSU H T, LEE T Y, et al. Naringenin,a dietary flavanone,enhances insulin-like growth factor 1 receptor-mediated antioxidant defense and attenuates methylglyoxal-induced neurite damage and apoptotic death[J]. Nutritional Neuroscience, 2021, 24(1):71-81.

[61]
HUANG B, HU P, HU A L, et al. Naringenin attenuates carotid restenosis in rats after balloon injury through its anti-inflammation and anti-oxidative effects via the RIP1-RIP3-MLKL signaling pathway[J]. European Journal of Pharmacology, 2019, 855:167-174.

DOI PMID

[62]
LI W S, LIN S C, CHU C H, et al. The gastroprotective effect of naringenin against ethanol-induced gastric ulcers in mice through inhibiting oxidative and inflammatory responses[J]. International Journal of Molecular Sciences, 2021, 22(21):11985.

[63]
裴素俭. 宠物犬肥胖的危害及防治措施[J]. 兽医导刊, 2020(21):116-117.

PEI S J. Harm and prevention measures of pet dog obesity[J]. Veterinary Orientation, 2020(21):116-117. (in Chinese)

[64]
BURKE A C, TELFORD D E, EDWARDS J Y, et al. Naringenin supplementation to a chow Diet enhances energy expenditure and fatty acid oxidation, and reduces adiposity in lean,pair-fed Ldlr-/- mice[J]. Molecular Nutrition & Food Research, 2019, 63(6):e1800833.

[65]
LIU H, ZHAO H, CHE J J, et al. Naringenin protects against hypertension by regulating lipid disorder and oxidative stress in a rat model[J]. Kidney & Blood Pressure Research, 2022, 47(6):423-432.

[66]
YOSHIDA H, WATANABE H, ISHIDA A, et al. Naringenin suppresses macrophage infiltration into adipose tissue in an early phase of high-fat diet-induced obesity[J]. Biochemical and Biophysical Research Communications, 2014, 454(1):95-101.

DOI PMID

[67]
TSUHAKO R, YOSHIDA H, SUGITA C, et al. Naringenin suppresses neutrophil infiltration into adipose tissue in high-fat diet-induced obese mice[J]. Journal of Natural Medicines, 2020, 74(1):229-237.

DOI PMID

[68]
ZHANG J A, ZHAO L, CHENG Q, et al. Structurally different flavonoid subclasses attenuate high-fat and high-fructose diet induced metabolic syndrome in rats[J]. Journal of Agricultural and Food Chemistry, 2018, 66(46):12412-12420.

DOI PMID

[69]
YANG Y, WU Y, ZOU J, et al. Naringenin attenuates non-alcoholic fatty liver disease by enhancing energy expenditure and regulating autophagy via AMPK[J]. Frontiers in Pharmacology, 2021, 12:687095.

[70]
RICHARD A J, AMINI-VAUGHAN Z, RIBNICKY D M, et al. Naringenin inhibits adipogenesis and reduces insulin sensitivity and adiponectin expression in adipocytes[J]. Evidence-Based Complementary and Alternative Medicine, 2013, 2013:549750.

[71]
BAWAZEER N A, CHOUDARY H, ZAMZAMI M A, et al. Possible regulation of LDL-receptor by naringenin in HepG2 hepatoma cell line[J]. African Journal of Traditional,Complementary,and Alternative Medicines, 2017, 14(1):278-287.

[72]
KE J Y, KLIEWER K L, HAMAD E M, et al. The flavonoid,naringenin,decreases adipose tissue mass and attenuates ovariectomy-associated metabolic disturbances in mice[J]. Nutrition & Metabolism, 2015, 12:1.

[73]
XIONG H H, LIN S Y, CHEN L L, et al. The interaction between flavonoids and intestinal microbes:a review[J]. Foods (Basel,Switzerland), 2023, 12(2):320.

[74]
WANG D F, ZHOU L L, ZHOU H L, et al. Chemical composition and protective effect of guava (Psidium guajava L.) leaf extract on piglet intestines[J]. Journal of the Science of Food and Agriculture, 2021, 101(7):2767-2778.

[75]
ZHONG J, YU R Y, ZHOU Q, et al. Naringenin prevents TNF-α-induced gut-vascular barrier disruption associated with inhibiting the NF-κB-mediated MLCK/p-MLC and NLRP3 pathways[J]. Food & Function, 2021, 12(6):2715-2725.

[76]
LEE S H, SEO D J, LEE K H, et al. Biometabolites of Citrus unshiu peel enhance intestinal permeability and alter gut commensal bacteria[J]. Nutrients, 2023, 15(2):319.

[77]
FARZAEI M H, RAHIMI R, ABDOLLAHI M. The role of dietary polyphenols in the management of inflammatory bowel disease[J]. Current Pharmaceutical Biotechnology, 2015, 16(3):196-210.

DOI PMID

[78]
FIRRMAN J, LIU L S, ARGOTY G A, et al. Analysis of temporal changes in growth and gene expression for commensal gut microbes in response to the polyphenol naringenin[J]. Microbiology Insights, 2018, 11:1178636118775100.

[79]
ZHAO Y C, YU S Q, LI L X, et al. Feeding citrus flavonoid extracts decreases bacterial endotoxin and systemic inflammation and improves immunometabolic status by modulating hindgut microbiome and metabolome in lactating dairy cows[J]. Animal Nutrition, 2023, 13:386-400.

DOI PMID

[80]
MEHDIPOUR M, DAGHIGH KIA H, NAJAFI A, et al. Effect of crocin and naringenin supplementation in cryopreservation medium on post-thaw rooster sperm quality and expression of apoptosis associated genes[J]. PLoS One, 2020, 15(10):e241105.

[81]
TVRDÁ E, DEBACKER M, ĎURAČKA M, et al. Quercetin and naringenin provide functional and antioxidant protection to stored boar semen[J]. Animals, 2020, 10(10):1930.

[82]
LIEN T F, YEH H S, SU W T. Effect of adding extracted hesperetin,naringenin and pectin on egg cholesterol,serum traits and antioxidant activity in laying hens[J]. Archives of Animal Nutrition, 2008, 62(1):33-43.

[83]
POAPOLATHEP A, POAPOLATHEP S, SUGITA-KONISHI Y, et al. The effect of naringenin on the fate and disposition of deoxynivalenol in piglets[J]. Journal of Veterinary Medical Science, 2010, 72(10):1289-1294.

PMID

[84]
NIU K M, WANG H Y, KIM S K, et al. Stepwise co-fermented traditional Chinese medicine byproducts improve antioxidant and anti-inflammatory effects in a piglet model[J]. Journal of the Science of Food and Agriculture, 2024, 104(2):1166-1177.

[85]
BURMAÑCZUK A, WOJCIECHOWSKA B, GBYLIK-SIKORSKA M, et al. The effect of hesperidin,chrysin,and naringenin on somatic cell count in mastitis dairy cows after multiple intramammary administration[J]. Annals of Animal Science, 2022, 22(1):155-172.

[86]
YU S Q, LI L X, ZHAO H Y, et al. Dietary citrus flavonoid extract improves lactational performance through modulating rumen microbiome and metabolites in dairy cows[J]. Food & Function, 2023, 14(1):94-111.

文章导航

/