研究论文

稻蛙种养模式下放养密度对黑斑蛙生长性能、血清激素和抗氧化指标及肠道菌群的影响

  • 韩光明 , 1, 2 ,
  • 覃宝利 1, 2 ,
  • 吴雷明 1, 2 ,
  • 张家宏 1, 2 ,
  • 寇祥明 , 1, 2, * ,
  • 王守红 1 ,
  • 徐荣 1, 2 ,
  • 马林杰 1, 2
展开
  • 1 江苏里下河地区农业科学研究所,扬州 225007
  • 2 江苏省生态农业工程技术研究中心,扬州 225007
*寇祥明,研究员,E-mail:

韩光明(1985—),男,江苏东海人,副研究员,硕士,研究方向为水产动物繁育与营养。E-mail:

Copy editor: 菅景颖

收稿日期: 2024-08-05

  网络出版日期: 2025-02-16

基金资助

扬州市生态农业重点实验室(YZ2023244)

Effects of Stocking Density on Growth Performance, Serum Hormones and Antioxidant Indicators, and Intestinal Flora of Dark-Spotted Frogs in Rice-Frog Coculture System

  • HAN Guangming , 1, 2 ,
  • QIN Baoli 1, 2 ,
  • WU Leiming 1, 2 ,
  • ZHANG Jiahong 1, 2 ,
  • KOU Xiangming , 1, 2, * ,
  • WANG Shouhong 1 ,
  • XU Rong 1, 2 ,
  • MA Linjie 1, 2
Expand
  • 1 Agricultural Science Institute of Jiangsu Lixiahe District, Yangzhou 225007, China
  • 2 Research Center for Eco-Agricultural Engineering and Technology of Jiangsu Province, Yangzhou 225007, China
*professor, E-mail:

Received date: 2024-08-05

  Online published: 2025-02-16

摘要

本试验旨在研究稻蛙种养模式下放养密度对黑斑蛙生长性能、血清激素和抗氧化指标及肠道菌群的影响。以初始体重为(8.12±0.03) g的黑斑蛙幼蛙为研究对象,设置5个放养密度,M1、M2、M3、M4、M5组放养密度分别为6、12、24、48和96只/m2(即0.4万、0.8万、1.6万、3.2万和6.4万只/亩),每组3个重复,养殖80 d。结果显示:1)放养密度超过24只/m2时,黑斑蛙的成活率出现显著下降(P<0.05);M3组黑斑蛙的末均重、增重率和特定生长率最高,且饲料系数显著低于M4和M5组(P<0.05)。2)各组之间血清皮质醇、胰岛素样生长因子-Ⅰ、甲状腺素含量以及超氧化物歧化酶、谷胱甘肽过氧化物酶、过氧化氢酶活性与丙二醛含量无显著差异(P>0.05),但M3组的血清总抗氧化能力显著高于M5组(P<0.05)。3)随着黑斑蛙放养密度的增加,肠道菌群的Chao1、Faith_pd、Observed_species、Shannon指数均出现上升的趋势,其中M5组显著高于M1组(P<0.05)。4)在门水平上,与M1和M2组比较,M4组肠道菌群中厚壁菌门(Firmicutes)的相对丰度显著下降(P<0.05),拟杆菌门(Bacteroidetes)的相对丰度显著升高(P<0.05);在属水平上,随着黑斑蛙放养密度的增加,肠道菌群中拟杆菌属(Bacteroides)的相对丰度呈上升趋势,乳球菌属(Lactococcus)的相对丰度呈下降趋势,罗姆布茨菌属(Romboutsia)和阿克曼菌属(Akkermansia)的相对丰度呈先上升后下降的趋势。综上可知,在本试验条件下,黑斑蛙放养密度过高不利于个体生长,适当增加放养密度可以提高肠道菌群多样性;在稻蛙种养模式下,建议黑斑蛙的放养密度为12~24只/m2(即0.8万~1.6万只/亩)。

本文引用格式

韩光明 , 覃宝利 , 吴雷明 , 张家宏 , 寇祥明 , 王守红 , 徐荣 , 马林杰 . 稻蛙种养模式下放养密度对黑斑蛙生长性能、血清激素和抗氧化指标及肠道菌群的影响[J]. 动物营养学报, 2025 , 37(2) : 1162 -1172 . DOI: 10.12418/CJAN2025.101

Abstract

This experiment aimed to study the effects of stocking density on the growth performance, serum hormones and antioxidant indicators, and intestinal flora of dark-spotted frogs (Pelophylax nigromaculatus) in rice-frog coculture system. Dark-spotted froglets with initial body weight of (8.12±0.03) g were cultured at five different stocking densities of 6, 12, 24, 48 and 96 frogs per square meter, further referred to as M1, M2, M3, M4 and M5 groups, with three replicates in each group, and the frogs were cultured for 80 days. The results showed as follows: 1) the survival rate of dark-spotted frogs significantly decreased with the stocking density exceeded 24 frogs per square meter. The average final weight, weight gain rate, and specific growth rate of dark-spotted frogs in group M3 were the highest, and the feed conversion ratio was significantly lower than that in groups M4 and M5 (P<0.05). 2) There were no significant differences in serum cortisol, insulin-like growth factor-Ⅰ, thyroid hormone contents, as well as superoxide dismutase, glutathione peroxidase, catalase activities and malondialdehyde content among the groups (P>0.05), but the serum total antioxidant capacity in group M3 was significantly higher than that in group M5 (P<0.05). 3) With the increase of stocking density of dark-spotted frogs, there was a trend of increase in the Chao1, Faith_pd, Observed_species, and Shannon’s indexes of the intestinal flora, which were significantly higher in M5 group than that in M1 group (P<0.05). 4) At the phylum level, the relative abundance of Firmicutes in the intestinal flora in the M4 group decreased significantly (P<0.05), and the relative abundance of Bacteroidetes in the M4 group increased significantly (P<0.05) compared with the M1 and M2 groups. At the genus level, with the increase of stocking density of dark-spotted frogs, the relative abundance of Bacteroides in the intestinal flora showed an increasing trend, the relative abundance of Lactococcus showed a decreasing trend, and the relative abundance of Romboutsia and Akkermansia showed a trend of increasing and then decreasing. In conclusion, under the conditions of this experiment, too high stocking density of dark-spotted frogs is unfavorable to individual growth, and an appropriate increase in stocking density can improve the diversity of intestinal flora. It is recommended that the stocking density of dark-spotted frogs should be 12 to 24 frogs per square meter in the rice-frog coculture system.

黑斑蛙(Pelophylax nigromaculatus),学名黑斑侧褶蛙,是我国广泛分布的本土蛙类,主要栖息于平原或丘陵地区的稻田、池塘、湖沼区及海拔2 200 m以下的山地。黑斑蛙虽然分布区很宽,但因栖息地的生态环境下降和过度捕捉,其种群数量急剧减少[1]。我国大部分地区居民都有吃蛙类的习惯,蛙肉味美且营养丰富,市场需求量大。因此,蛙类人工驯养是解决供需矛盾、保护蛙类资源的必由之路[2]。2020年,国家明确了对养殖蛙类的管控,人工养殖的黑斑蛙由渔业主管部门按照水生动物管理[3]。稻蛙种养模式作为近年来兴起的一种新型稻田综合种养模式,在中国南方稻区及长江流域具有良好的发展态势[4]。从经济效益及成本核算上来看,相对于其他的稻田综合种养模式来说,稻蛙模式更具挖掘潜力,更具推广意义,定将成为一种理想的稻田综合种养模式[5]
放养密度是决定养殖动物生长性能和生存能力的关键因素,也是总体生产效率和成本效益的关键决定因素。在稻蛙种养模式中,蛙类活动和排泄有利于改善土壤养分状况,稻蛙种养模式中减施化肥或不施肥,水稻也可以获得较高产量[6]。但是在实际生产中养殖户为了追求高产,黑斑蛙放养密度过高,会导致黑斑蛙成活率、养成规格下降,也会致使稻田肥力偏高,对土壤和水环境产生负面影响[7]。已有研究表明,高放养密度会引起养殖环境和动物行为的改变,使动物机体的应激反应增多,对动物生理稳态(激素分泌、抗氧化能力、免疫功能、营养物质代谢和肠道功能)产生负面影响,最终导致动物疾病发生率升高,生产性能下降[8]。目前,在稻蛙种养模式中,关于黑斑蛙适宜放养密度的报道,大多来自生产技术总结,相关报道的结果有一定的差异[9-11],关于放养密度对黑斑蛙生理代谢、肠道健康等方面的研究探讨尚少。本研究探讨了放养密度对黑斑蛙生长性能、血清激素和抗氧化指标及肠道菌群的影响,旨在进一步探讨稻蛙种养模式下黑斑蛙的合理放养密度,为黑斑蛙的养殖生产提供参考。

1 材料与方法

1.1 试验材料

试验所用黑斑蛙幼蛙购买自当地养殖场[驯养繁殖许可文号:苏(扬)发驯繁2018008号],挑选健康无畸形、活力强、大小相近的幼蛙用于试验,平均体质量为(8.12±0.03) g/只。试验所用水稻品种为南粳5055,水稻秧苗采用秧盘育秧,秧龄20 d后进行移栽。

1.2 试验地点和试验条件

试验地点为江苏里下河地区农业科学研究所高邮基地。模拟稻蛙共作生产要求改造出试验田块15个,每个田块面积7.5 m2,其中稻田面积占90%、黑斑蛙食台面积占10%,田块四周设置防逃膜,上方设置防鸟网。水稻于2023年7月3日移栽,行株距为30 cm×14 cm,每穴4苗。每个田块施用基肥:303.75 g复合肥(N∶P2O5∶K2O=15∶15∶15),分蘖肥:101.25 g尿素(总氮含量≥46.4%),即每亩(1亩≈667 m2)施用复合肥30 kg、尿素10 kg。

1.3 试验设计和试验管理

动物试验按照《实验动物管理条例》进行,并执行江苏省农业科学院动物福利和伦理委员会的规定。设置5个放养密度,M1、M2、M3、M4、M5组黑斑蛙幼蛙放养密度分别为6、12、24、48和96只/m2(折算成每亩放养密度为0.4万、0.8万、1.6万、3.2万和6.4万只/亩),每组3个重复。在水稻移栽后20 d,按照放养密度设计投放黑斑蛙幼蛙,投喂黑斑蛙商品膨化配合饲料(粗蛋白质含量40%、粗脂肪含量5%),每日2次。根据当日摄食情况,调节次日投喂量,养殖80 d(2023年7月23日至2023年10月11日)。

1.4 样品采集及指标检测方法

黑斑蛙养殖结束时禁食24 h,捕出各组黑斑蛙进行逐个称重。每个试验田块随机选取黑斑蛙6只,抽取血液,立即离心(2 200×g,10 min),吸取上清液置于-80 ℃保存,用于血清激素和抗氧化指标检测。采用双毁髓法将黑斑蛙处死解剖,取出肠道并收集肠道内容物,放入液氮后转移至-80 ℃保存,用于肠道菌群检测。
生长性能指标计算公式如下:
成活率(survival rate,SR,%)=100×Nf/Ni;
增重率(weight gain ratio,WGR,%)=100×(Wf-Wi)/Wi;
特定生长率(specific growth ratio,SGR,%/d)=100×(lnWf-lnWi)/D;
饲料系数(feed conversion ratio,FCR)=F/(Wf-Wi);
肝体指数(hepatosomatic index,HSI,%)=100×Wh/W;
后腿指数(hind leg index,HLI,%)=100×Wl/W
式中:Nf为试验末蛙数量(g);Ni为试验初蛙数量(g);Wf为试验末蛙体重量(g);Wi为试验初蛙体重量(g);D为饲养天数(d);F为摄入的饲粮干重(g);Wh为蛙肝脏重量(g);Wl为蛙后腿重量(g);W为对应的蛙体重量(g)。
血清样品送至南京建成生物工程研究所,采用酶联免疫吸附试验法检测血清皮质醇(cortisol,COR)、胰岛素生长因子-Ⅰ(insulin-like growth factor-Ⅰ,IGF-Ⅰ)、甲状腺素(thyroxine,T4)等激素的水平,分别采用羟胺法、硫代巴比妥酸法、比色法、可见光法和铁离子还原/抗氧化能力法测定血清超氧化物歧化酶(superoxide dismutase,SOD)、丙二醛(malondialdehyde,MDA)、谷胱甘肽过氧化物酶(glutathione peroxidase,GSH-Px)、过氧化氢酶(catalase,CAT)和总抗氧化能力(total antioxidant capacity,T-AOC)等抗氧化指标。
将肠道内容物样品送至上海派森诺生物科技股份有限公司进行肠道菌群的测定和分析,每组测定4个样本。肠道微生物DNA提取使用OMEGA Soil DNA Kit(D5625-01,Omega Bio-Tek,美国)。使用引物338F(5'-ACTCCTACGGGAGGCAGCA-3')和806R(5'-GGACTACHVGGGTWTCTAAT-3')对微生物16S rRNA基因V3~V4区进行扩增,扩增区域长度约500 bp,通过Illumina MiSeq平台进行高通量双末端测序。生物信息分析在派森诺基因云(https://www.genescloud.cn/home)完成。使用Uparse软件以97%的相似性进行操作分类单元(operational taxonomic units,OTUs)聚类。使用QIIME(1.7.0版)软件分析肠道菌群α多样性,在各个分类水平上进行菌群组成和差异分析。利用PICRUSt菌群代谢功能预测工具与基因功能谱数据库进行比对,推测微生物群落的功能类别丰度信息。

1.5 数据统计与分析

采用SPSS 19.0统计软件中的单因素方差分析(one-way ANOVA)程序对数据进行统计分析,若达到显著差异,则进行Fisher’s LSD多重比较。数据用平均值±标准误(mean±SE)形式表示,P<0.05认为差异显著。

2 结果与分析

2.1 放养密度对黑斑蛙生长性能的影响

表1可知,黑斑蛙的成活率随放养密度的增加呈下降趋势,其中M3、M4和M5组均显著低于M1、M2组(P<0.05);黑斑蛙的末均重、增重率和特定生长率的最高值均出现在M3组,且均显著高于M1、M4和M5组(P<0.05);M4和M5组的饲料系数均显著高于M1、M2和M3组(P<0.05),同时M1、M2和M3组之间无显著差异(P>0.05);各组黑斑蛙的肝体指数无显著差异(P>0.05);M1组的后腿指数显著高于M5组(P<0.05),其他组之间无显著差异(P>0.05)。
表1 放养密度对黑斑蛙生长性能的影响

Table 1 Effects of stocking density on growth performance of dark-spotted frogs

项目
Items
组别Groups P
P-value
M1 M2 M3 M4 M5
成活率SR/% 95.56±2.22a 96.67±1.11a 86.39±0.83b 77.78±3.89c 65.07±1.46d <0.001
末均重FBW/g 30.81±0.12b 31.31±0.21a 31.38±0.08a 29.59±0.20c 24.34±0.03d 0.001
增重率WGR/% 279.49±1.53b 285.54±2.53ab 286.42±1.04a 264.43±2.48c 199.73±0.35d <0.001
特定生长率SGR/(%/d) 1.67±0.01b 1.69±0.01ab 1.69±0.00a 1.62±0.01c 1.37±0.00d <0.001
饲料系数FCR 1.66±0.10c 1.66±0.10c 1.82±0.02c 2.16±0.08b 2.55±0.07a 0.002
肝体指数HSI/% 5.37±0.48 5.25±0.28 6.64±0.43 6.00±0.87 5.77±0.63 0.354
后腿指数HLI/% 36.51±0.42a 35.46±0.81ab 34.54±0.57ab 34.98±0.64ab 34.45±1.04b 0.049

同行数据肩标无字母或相同字母表示差异不显著(P>0.05),不同小写字母表示差异显著(P<0.05)。下表同。

In the same row, values with no letter or the same letter superscripts mean no significant difference (P>0.05), while with different small letter superscripts mean significant difference (P<0.05). The same as below.

2.2 放养密度对黑斑蛙血清激素和抗氧化指标的影响

表2可知,黑斑蛙血清COR、IGF-Ⅰ、T4水平各组之间未观察到显著差异(P>0.05),但M4和M5组血清IGF-Ⅰ水平较低。黑斑蛙血清SOD、GSH-Px、CAT活性和MDA含量无显著差异(P>0.05);M3组黑斑蛙血清T-AOC显著高于M5组(P<0.05),其他组之间无显著差异(P>0.05)。
表2 放养密度对黑斑蛙血清激素和抗氧化指标的影响

Table 2 Effects of stocking density on serum hormone and antioxidant indexes of dark-spotted frogs

项目
Items
组别Groups P
P-value
M1 M2 M3 M4 M5
皮质醇COR/(ng/mL) 19.12±0.54 21.95±0.43 21.31±1.62 21.78±0.71 20.70±0.44 0.238
胰岛素生长因子-Ⅰ
IGF-Ⅰ/(ng/mL)
26.55±3.97 26.74±7.40 27.11±1.04 24.14±1.13 24.36±0.40 0.935
甲状腺素T4/(ng/mL) 56.66±3.35 67.60±0.39 54.40±7.14 52.21±4.99 54.89±4.09 0.310
超氧化物歧化酶
SOD/(U/mL)
316.86±10.13 303.07±13.51 322.75±20.93 291.30±27.82 267.78±13.84 0.283
丙二醛MDA/(nmol/mL) 4.78±0.49 6.41±1.09 6.69±0.09 5.49±0.43 5.97±0.50 0.144
谷胱甘肽过氧化物酶
GSH-Px/(U/mL)
247.83±5.92 256.23±36.61 297.39±25.42 245.22±14.86 267.83±26.38 0.480
过氧化氢酶CAT/(U/mL) 15.57±2.85 17.10±0.52 17.95±3.45 18.15±5.87 13.69±2.72 0.898
总抗氧化能力
T-AOC/(mmol/L)
1.24±0.05ab 1.34±0.15ab 1.42±0.05a 1.27±0.13ab 1.18±0.02b 0.013

2.3 放养密度对黑斑蛙肠道菌群多样性的影响

选取Chao1、Faith_pd、Observed_species、Pielou_e、Shannon和Simpson指数反映黑斑蛙肠道菌群的α多样性,结果(表3)显示,随着黑斑蛙放养密度的增加,Chao1、Faith_pd、Observed_species、Shannon指数均出现上升的趋势,且高放养密度组(M5组)显著高于低放养密度组(M1组)(P<0.05),即肠道菌群物种种类更丰富、多样性更高;各组之间Pielou_e和Simpson指数无显著差异(P>0.05),说明肠道菌群物种数量分布均匀,优势种的地位不突出。
表3 各组黑斑蛙肠道菌群α多样性指数

Table 3 Alpha diversity indexes of intestinal flora of dark-spotted frogs in different groups

项目
Items
组别Groups P
P-value
M1 M2 M3 M4 M5
Chao1指数Chao1 index 704.46±95.86b 635.90±33.84b 1 018.10±162.18a 1 058.46±61.30a 1 101.94±103.58a 0.013
Faith_pd指数Faith_pd index 57.94±8.41b 55.15±3.41b 72.38±9.07ab 68.18±1.90ab 80.57±5.12a 0.046
Observed_species指数
Observed_species index
677.53±92.12b 611.28±35.13b 972.48±159.17ab 1 038.40±62.02a 1 077.08±108.93a 0.013
Pielou_e指数Pielou_e index 0.60±0.04 0.59±0.00 0.64±0.03 0.62±0.04 0.67±0.02 0.472
Shannon指数Shannon index 5.65±0.45b 5.48±0.08ab 6.34±0.31ab 6.25±0.42ab 6.70±0.34a 0.048
Simpson指数Simpson index 0.91±0.04 0.93±0.01 0.95±0.02 0.92±0.04 0.96±0.01 0.761

2.4 放养密度对黑斑蛙肠道菌群组成的影响

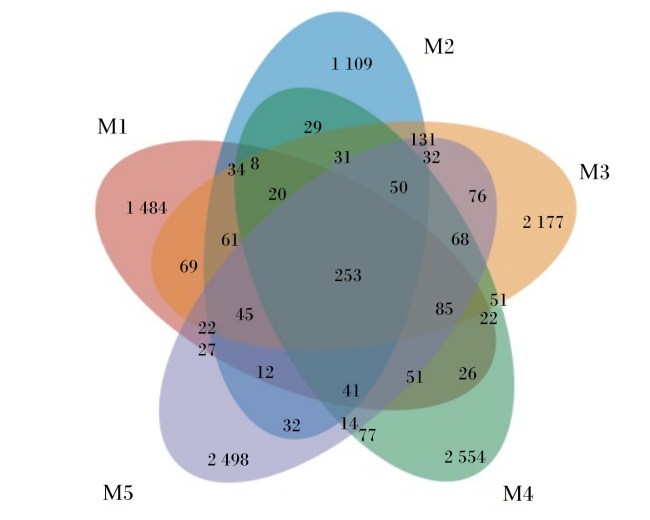
韦恩图(图1)显示了不同放养密度组黑斑蛙肠道菌群共有的与独有的OTUs数量,从图中可以看出,M4、M5组肠道菌群的OTUs数量远高于M1和M2组;5组样本共享的OTUs有253个,占全部OTUs的2.26%;M1、M2、M3、M4和M5组独有的OTUs数量分别为1 484、1 109、2 177、2 554和2 498个,随着放养密度增加,黑斑蛙肠道菌群OTUs数量呈现上升的趋势。
图1 各组黑斑蛙肠道菌群OTUs的韦恩图

M1:M1组 M1 group;M2:M2组 M2 group;M3:M3组 M3 group;M4:M4组 M4 group;M5:M5组 M5 group。

Fig.1 Venn diagram of OTUs for intestinal flora of dark-spotted frogs in different groups

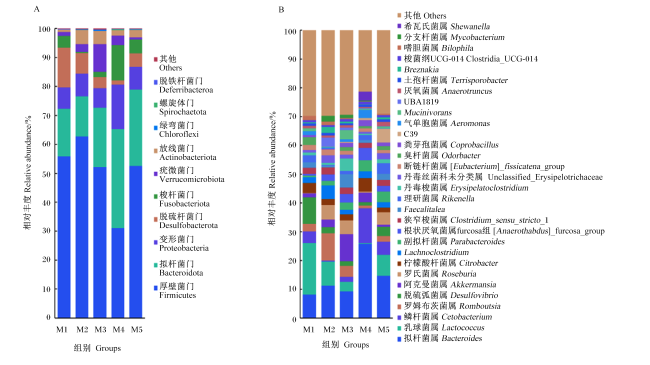
在黑斑蛙肠道菌群中鉴定出的34个菌门,主要菌门为厚壁菌门(Firmicutes)、拟杆菌门(Bacteroidota)、变形菌门(Proteobacteria)、脱硫杆菌门(Desulfobacterota)、梭杆菌门(Fusobacteriota)、疣微菌门(Verrucomicrobiota)、放线菌门(Actinobacteriota),其余27个门相对丰度均小于0.5%(图2-A)。厚壁菌门、拟杆菌门、变形菌门和脱硫杆菌门是各组的优势菌群,相对丰度为82.06%~93.39%,其中与M1和M2组比较,M4组厚壁菌门相对丰度显著下降(P<0.05),拟杆菌门相对丰度显著升高(P<0.05),另外,M4组脱硫杆菌门丰度显著低于M1组(P<0.05),各组之间其他菌门的相对丰度未观察到显著差异(P>0.05)(表4)。
图2 各组黑斑蛙肠道菌群组成分析(A:门水平;B:属水平)

Fig.2 Analysis of intestinal flora composition of dark-spotted frogs in different groups (A: phylum level; B: genus level)

表4 黑斑蛙肠道菌群中的差异菌门和菌属(相对丰度)

Table 4 Differential phyla and genera in intestinal flora of dark-spotted frogs (relative abundance) %

项目
Items
组别Groups P
P-value
M1 M2 M3 M4 M5
门水平Phylum level
厚壁菌门Firmicutes 55.81±6.06a 62.70±7.87a 52.15±11.60ab 30.99±5.38b 52.49±6.65ab 0.040
拟杆菌门Bacteroidota 16.51±0.62b 13.93±9.56b 20.46±5.70ab 34.34±4.38a 26.37±5.99ab 0.029
脱硫杆菌门Desulfobacterota 13.68±7.70a 7.10±4.10ab 3.80±1.59ab 1.43±0.49b 4.66±0.37ab 0.046
属水平Genus level
拟杆菌属Bacteroides 8.13±2.85b 11.19±10.3ab 9.27±3.91ab 25.81±5.52a 14.67±3.15ab 0.049
罗姆布茨菌属Romboutsia 2.50±1.89ab 9.51±5.45a 3.86±2.08b 0.93±0.38b 1.93±1.09ab 0.046
在属水平上(图2-B),黑斑蛙肠道菌群中的主要菌属有拟杆菌属(Bacteroides)、乳球菌属(Lactococcus)、鲸杆菌属(Cetobacterium)、罗姆布茨菌属(Romboutsia)、脱硫弧菌属(Desulfovibrio)、阿克曼菌属(Akkermansia)、罗氏菌属(Roseburia)、柠檬酸杆菌属(Citrobacter),在M1、M2、M3、M4和M5组中的相对丰度分别为46.91%、41.37%、36.05%、48.65%和38.36%。随着黑斑蛙放养密度的增加,拟杆菌属相对丰度呈上升趋势,乳球菌属相对丰度呈下降趋势,罗姆布茨菌属和阿克曼菌属相对丰度呈先上升后下降的趋势,其中M4组的拟杆菌属相对丰度(25.81%)显著高于M1组(8.13%),罗姆布茨菌属(0.93%)相对丰度显著低于M2组(9.51%),其他菌属的相对丰度在不同放养密度组中有一定的差异,但是方差分析未产生显著差异(P>0.05)(表4)。

2.5 黑斑蛙肠道菌群功能潜能预测分析

肠道菌群功能潜能预测分析见表5。在KEGG数据库第1等级代谢通路中,黑斑蛙肠道菌群的功能主要集中于生物合成、降解/利用/同化、前体代谢产物和能量的产生,且它们的相对丰度在各组之间无显著差异(P<0.05);M3组的聚糖途径相对丰度显著高于M1组(P<0.05),其他各组之间无显著差异(P>0.05)。
表5 KEGG代谢通路统计

Table 5 Metabolic pathway statistics based on KEGG

项目
Items
组别Groups P
P-value
M1 M2 M3 M4 M5
生物合成Biosynthesis 161 817±2 479 156 281±4 483 164 237±3 815 162 404±6 045 163 792±3 933 0.703
降解/利用/同化
Degradation/utilization/
assimilation
38 951±4 810 44 217±2 956 40 809±2 593 43 350±2 386 41 392±1 359 0.754
解毒Detoxification 1 026±323 1 098±278 916±158 503±87 1 002±307 0.486
前体代谢产物和能量的产生
Generation of precursor
metabolite and energy
28 706±1967 30 605±851 29 809±2 345 30 658±2 485 31 030±1 920 0.926
聚糖途径Glycan pathways 2 608±94b 2 948±82ab 3 083±216a 2 951±87ab 2 949±147ab 0.025
大分子修饰
Macromolecule modification
1 263±163 999±175 1 152±202 1 347±239 1 299±37 0.655
代谢簇Metabolic clusters 6 838±504 6 841±71 7 688±84 7 090±332 7 308±187 0.238

3 讨论

3.1 放养密度对黑斑蛙生长性能及产量的影响

放养密度是动物养殖生产的关键参数,当以养殖产量最大化为生产目标时,增加放养密度可以优化成本和空间,提高养殖利润[12]。在本试验条件下,当黑斑蛙放养密度为1.6万只/亩时,与低放养密度组(0.4万只/亩)相比,成活率虽然下降,但是末均重、增重率和特定生长率均显著提高,说明黑斑蛙低密度养殖不一定获得较高的生长速度,在北极红点鲑(Salvelinus alpinus)[13]和欧洲鲈鱼(Dicentrarchus labrax)[14]上也出现了类似的结果。当养殖密度过高时,普遍认为会对养殖动物产生胁迫,在水产动物上的研究表明,高密度养殖会对养殖动物的生长性能和成活产生负面影响[15-17]。本试验发现,当黑斑蛙放养密度达到3.2万只/亩以及以上时,成活率和生长性能均显著下降,饲料系数显著升高。然而,有一些物种可以耐受高密度养殖,例如金鱼(Carassius auratus),其生长和存活在高密度养殖下未出现负面影响[18]。也有学者通过研究不同养殖密度下大西洋鲑和虹鳟的生长表现,认为养殖密度对鱼类生长并无直接影响,而是通过密度的改变对养殖水质产生影响,从而间接影响鱼类生长[19]
在稻蛙种养模式下黑斑蛙适宜放养密度的研究方面,金晶等[9]报道,黑斑蛙放养密度为2万~3万只/亩时,成蛙产量可达555.6~837.6 kg/亩;孙益豪等[10]报道,黑斑蛙放养密度为3万只/亩时,可收获成蛙752.9 kg/亩;曾涛等[11]报道,黑斑蛙成活率随放养密度的增加而降低,贵州天柱县地区适宜放养密度为1万只/亩,黑斑蛙成活率为58.3%,产量达230.11 kg/亩,播州区适宜放养密度为0.5万只/亩,当放养密度为1.5万~2万只/亩时,容易导致成活率过低出现亏损。由此可见,不同研究者对黑斑蛙适宜放养密度的研究结果并不一致,其主要原因可能是养殖环境和管理水平不同,导致黑斑蛙的成活率差异较大。从本研究结果来看,稻蛙种养模式下黑斑蛙的适宜放养密度为0.8万~1.6万只/亩。

3.2 放养密度对黑斑蛙血清激素和抗氧化指标的影响

过高的养殖密度会引起动物机体多种激素分泌紊乱。有研究表明,高密度养殖引起鱼体血清COR水平显著升高,血清三碘甲状腺原氨酸和T4水平随着放养密度的增加而降低[20-21]。本试验并没有观察到高放养密度组中黑斑蛙血清COR水平升高,但观察到高放养密度组黑斑蛙血清中T4和IGF-Ⅰ水平呈下降的趋势,但是各组之间差异不显著,说明黑斑蛙对高密度养殖具有一定的耐受性,对高密度养殖的应激反应较小。
高密度胁迫作为一种慢性环境胁迫因子,也将会引起养殖动物产生氧化应激。动物机体具有广泛的抗氧化防御体系,以避免过量的自由基对机体造成损伤。高密度胁迫会引起SOD、CAT等抗氧化酶活性升高[20-22],这种明显的升高恰好是为了清除在压力条件下体内产生的过量超氧化物。本研究结果显示,6.4万只/亩放养密度组黑斑蛙的血清T-AOC显著低于1.6万只/亩密度组,高放养密度导致血清总抗氧化活力下降,这一结果与在其他养殖动物上的结果[23-25]相似。此外,黑斑蛙血清SOD、CAT、GSH-Px活性以及MDA含量在不同放养密度组中无显著差异,表明高放养密度引起了适度的氧化应激,其产生的影响可能在黑斑蛙机体的耐受范围之内。

3.3 放养密度对黑斑蛙肠道菌群结构和功能的影响

肠道菌群作为动物体不可忽视的重要组成部分,在促进水产动物生长发育、提高抗病力以及应对环境胁迫等方面起着关键作用[26]。蛙类肠道菌群结构受内源性(如遗传、生命阶段)和外源性(如饮食、生境条件)因素影响,处于动态变化之中[27]。本研究结果表明,随着黑斑蛙放养密度的增加,Chao1、Faith_pd、Observed_species、Shannon指数均显著提高,肠道菌群的α多样性水平提高,这可能是因为放养密度改变了环境中的微生物组成,间接提高了肠道菌群多样性,在稻鱼种养的研究中也发现了相似结果[28]
本研究结果显示,各组黑斑蛙肠道菌群中的优势菌门均为厚壁菌门、拟杆菌门、变形菌门和脱硫杆菌门,这与已经报道的黑斑蛙肠道优势菌群的结果[27,29]基本相近,与鱼类[30]也有一定的相似度。放养密度能够使养殖动物肠道菌群结构发生显著变化,而肠道菌群失衡对养殖动物会产生不利的影响[31-32]。本研究发现,高放养密度组(3.2万只/亩)黑斑蛙肠道菌群中厚壁菌门的相对丰度显著下降、拟杆菌门的相对丰度显著升高,随着放养密度的增加,厚壁菌门与拟杆菌门的比值呈下降的趋势,该比值的高低与黑斑蛙的体重呈正相关,由此可见,放养密度增加导致黑斑蛙生长性能下降,可能会间接导致厚壁菌门与拟杆菌门比值下降。养殖环境中残留饵料及养殖动物粪便在水体中未被及时分解并沉积在水体及底泥中时,会造成养殖池塘底部拟杆菌门细菌数量增加[33],因此,高密度放养组黑斑蛙肠道菌群中拟杆菌门相对丰度增加也有可能是环境中拟杆菌门细菌过多导致。本研究发现,在属水平上,高放养密度组(3.2万只/亩)黑斑蛙肠道菌群中拟杆菌属的相对丰度显著升高,乳球菌属的相对丰度显著下降,但是在团头鲂上的研究发现,随着放养密度的增加,肠道菌群中拟杆菌属、乳球菌属的数量均显著减少[34]。由此可见,放养密度不同,动物肠道菌群结构的差异较大。
肠道菌群功能潜能预测分析结果显示,黑斑蛙肠道菌群的功能通路主要集中于生物合成功能。通过代谢通路差异分析,发现随着黑斑蛙放养密度的增加,聚糖途径相对丰度呈现先上升后下降的趋势,其中放养密度为1.6万只/亩时,聚糖途径相对丰度最高,这可能是与该组肠道中阿克曼菌属的相对丰度较高有关,有研究表明阿克曼菌属能够影响宿主的糖代谢[35]。有研究发现,高放养密度显著降低了凡纳滨对虾肠道菌群中N-聚糖生物合成能力,从而阻碍其生长发育[36-37]。由此可见,不同放养密度影响了黑斑蛙肠道菌群的功能。

4 结论

在本试验条件下,黑斑蛙放养密度过高不利于个体生长,适当增加放养密度可以提高肠道菌群多样性;在稻蛙种养模式下,建议黑斑蛙放养密度为12~24只/m2(即0.8万~1.6万只/亩)。
[1]
费梁, 叶昌媛, 江建平. 中国两栖动物及其分布彩色图鉴[M]. 成都: 四川科学技术出版社, 2012:324.

FEI L, YE C Y, JIANG J P. Colored atlas of Chinese amphibians and their distributions[M]. Chengdu: Sichuan Science and Technology Publishign House, 2012:324. (in Chinese)

[2]
李兴华, 涂军明, 陈展鹏, 等. 稻蛙绿色种养模式研究及其可持续发展策略[J]. 农学学报, 2020, 10(12):98-103.

DOI

LI X H, TU J M, CHEN Z P, et al. Rice-frog planting and raising mode and its sustainable development strategy[J]. Journal of Agriculture, 2020, 10(12):98-103. (in Chinese)

DOI

[3]
农业农村部, 国家林业和草原局. 农业农村部、国家林业和草原局关于进一步规范蛙类保护管理的通知[J]. 中华人民共和国农业农村部公报, 2020(7):20-21.

Ministry of Agriculture and Rural Affairs,National Forestry and Grassland Administration. Joint circular of the Ministry of Agriculture and Rural Affairs and the National Forestry and Grassland Administration on further regulating management of frog protection[J]. Gazette of the Ministry of Agriculture and Rural Affairs of the People’s Republic of China, 2020(7):20-21. (in Chinese)

[4]
刘伟玮, 闵庆文, 刘某承, 等. 不同稻田生态种养模式控制面源污染的效果研究[J]. 中国农学通报, 2014, 30(增刊):124-129.

LIU W W, MIN Q W, LIU M C, et al. Study on the effect of different ecological planting and breeding modes in controlling non-point source pollution in paddy fields[J]. Chinese Agricultural Science Bulletin, 2014, 30(Suppl.):124-129. (in Chinese)

[5]
韩洪波, 李星星, 赵谱远, 等. 稻蛙综合种养模式技术分析、存在问题与发展趋势[J]. 中国水产, 2018(3):83-84.

HAN H B, LI X X, ZHAO P Y, et al. Technical analysis,existing problems,and development trends of comprehensive planting and breeding model for rice frog[J]. China Fisheries, 2018(3):83-84. (in Chinese)

[6]
李金龙, 徐永福, 王冬武, 等. 黑斑蛙养殖模式对稻田土壤肥力、土壤酶活性的影响及其经济效益[J]. 作物研究, 2019, 33(5):428-431, 436.

LI J L, XU Y F, WANG D W, et al. Effects of breeding models of Rana nigromaculata on soil fertility and enzyme activity in paddy field and economic benefit analysis[J]. Crop Research, 2019, 33(5):428-431, 436. (in Chinese)

[7]
梁正其, 蔡蝶, 陈岚英, 等. 不同黑斑蛙蝌蚪放养密度对贵州山区稻蛙共生模式中黑斑蛙生长的影响[J]. 特产研究, 2024, 46(2):16-21.

LIANG Z Q, CAI D, CHEN L Y, et al. Effects of different stocking density on growth of Rana nigromaculata in rice-frog symbiosis in the mountainous area of Guizhou Province[J]. Special Wild Economic Animal and Plant Research, 2024, 46(2):16-21. (in Chinese)

[8]
左权, 杨开伦, 杨红建, 等. 饲养密度对动物生产的影响[J]. 动物营养学报, 2024, 36(1):141-150.

DOI

ZUO Q, YANG K L, YANG H J, et al. Effects of stocking density on animal production[J]. Chinese Journal of Animal Nutrition, 2024, 36(1):141-150. (in Chinese)

DOI

[9]
金晶, 贝亦江, 袁帆, 等. 不同放养密度对稻-黑斑蛙综合种养成效的影响[J]. 中国水产, 2024, 583(6):64-67.

JIN J, BEI Y J, YUAN F, et al. The effect of different stocking densities of Pelophylax nigromaculatus on the comprehensive breeding efficiency of rice-frog symbiosis[J]. China Fisheries, 2024, 583(6):64-67. (in Chinese)

[10]
孙益豪, 金涛, 张家宏. 稻-蛙鳅综合种养模式的技术集成及经济效益分析[J]. 江苏农业科学, 2021, 49(16):88-92.

SUN Y H, JIN T, ZHANG J H. Technical integration and economic benefit analysis of rice-frog loach integrated planting and breeding model[J]. Jiangsu Agricultural Sciences, 2021, 49(16):88-92. (in Chinese)

[11]
曾涛, 熊玉唐, 陈卓, 等. 贵州稻区稻蛙共生适宜的养蛙密度[J]. 贵州农业科学, 2019, 47(11):84-87.

ZENG T, XIONG Y T, CHEN Z, et al. Preliminary study of appropriate density of frog on rice-frog system in main rice planting areas of Guizhou[J]. Guizhou Agricultural Sciences, 2019, 47(11):84-87. (in Chinese)

[12]
YENGKOKPAM S, DAS B K, DEBNATH D, et al. Effect of stocking density on growth and yield of Labeo bata fingerlings reared in cages[J]. Aquaculture Reports, 2020, 18:100506.

[13]
JØRGENSEN E H, CHRISTIANSEN J S, JOBLING M. Effects of stocking density on food intake,growth performance and oxygen consumption in Arctic charr (Salvelinus alpinus)[J]. Aquaculture, 1993, 110(2):191-204.

[14]
PAPOUTSOGLOU S E, TZIHA G, VRETTOS X, et al. Effects of stocking density on behavior and growth rate of European sea bass (Dicentrarchus labrax) juveniles reared in a closed circulated system[J]. Aquacultural Engineering, 1998, 18(2):135-144.

[15]
LIN T T, LI S P, ZHANG D, et al. Effects of stocking density on the survival,growth,and stress levels of the juvenile lined seahorse (Hippocampus erectus) in recirculating aquaculture systems[J]. Biology, 2024, 13(10):807.

[16]
JIA R, LIU B L, FENG W R, et al. Stress and immune responses in skin of turbot (Scophthalmus maximus) under different stocking densities[J]. Fish & Shellfish Immunology, 2016, 55:131-139.

[17]
麻艳群, 司楠, 程蔓, 等. 放养密度对黄颡鱼生长、营养成分、消化及抗氧化性的影响[J]. 水产学杂志, 2024, 37(3):44-49.

MA Y Q, SI N, CHENG M, et al. Effects of stocking density on growth performance,nutrient composition,gigestion and antioxidant activity of yellow catfish Pelteobagrus fulvidraco[J]. Chinese Journal of Fisheries, 2024, 37(3):44-49. (in Chinese)

[18]
NIAZIE E H N, IMANPOOR M, TAGHIZADE V, et al. Effects of density stress on growth indices and survival rate of goldfish (Carassius auratus)[J]. Global Veterinaria, 2013, 10(3):365-371.

[19]
NORTH B P, TURNBULL J F, ELLIS T, et al. The impact of stocking density on the welfare of rainbow trout (Oncorhynchus mykiss)[J]. Aquaculture, 2006, 255(1/2/3/4):466-479.

[20]
UPADHYAY A, SWAIN H S, DAS B K, et al. Stocking density matters in open water cage culture:influence on growth,digestive enzymes,haemato-immuno and stress responses of Puntius sarana (Ham, 1822)[J]. Aquaculture, 2022, 547:737445.

[21]
ONXAYVIENG K, PIRIA M, FUKA M M, et al. High stocking density alters growth performance,blood biochemical profiles,and hepatic antioxidative capacity in gibel carp (Carassius gibelio)[J]. Fish Physiology and Biochemistry, 2021, 47(2):203-212.

[22]
KÖPRÜCÜ K, MISE YONAR S, KÖPRÜCÜ S, et al. Correction to:effect of different stocking densities on growth,oxidative stress,antioxidant enzymes,and hematological and immunological values of European catfish (Silurus glanis L.,1758)[J]. Aquaculture International, 2024, 32(3):2975-2975.

[23]
RONG Y R, LI B, HOU Y R, et al. Influences of stocking density on antioxidant status,nutrients composition,and lipid metabolism in the muscles of Cyprinus carpio under rice-fish co-culture[J]. Antioxidants, 2024, 13(7):849.

[24]
丁崇航, 贾睿, 侯诒然, 等. 稻鲈共作系统中养殖密度对大口黑鲈抗氧化状态、肌肉营养品质和代谢功能的影响[J]. 中国水产科学, 2023, 30(8):1000-1014.

DING C H, JIA R, HOU Y R, et al. Effects of stocking density on the antioxidant capacity,muscle nutrient composition and metabolism function of Micropterus salmoides in integrated rice-bass farming systems[J]. Journal of fishery sciences of China, 2023, 30(8):1000-1014. (in Chinese)

[25]
LIU B L, JIA R, HAN C, et al. Effects of stocking density on antioxidant status, metabolism and immune response in juvenile turbot (Scophthalmus maximus)[J]. Comparative Biochemistry and Physiology:Part C, 2016, 190:1-8.

[26]
赵新宇, 史宝, 程汉良, 等. 肠道菌群对水产动物重要经济性状影响的研究进展[J]. 水产学杂志, 2024, 37(3):100-108, 116.

ZHAO X Y, SHI B, CHENG H L, et al. Research progress on effect of gut microbiota on important economic traits of animals in aquaculture:a review[J]. Chinese Journal of Fisheries, 2024, 37(3):100-108,116. (in Chinese)

[27]
翟元圆. 稻蛙共作模式下黑斑侧褶蛙肠道菌群结构及其动态变化[D]. 硕士学位论文. 信阳: 信阳师范学院, 2021.

ZHAI Y Y. Structure dynamics of gut microbiota of Pelophylax nigromaculatus in rice-frog co-cultivation mode[D]. Master’s Thesis. Xinyang: Xinyang Normal University, 2021. (in Chinese)

[28]
DIAO W, JIA R, HOU Y, et al. Effects of different stocking densities on the growth,antioxidant status,and intestinal bacterial communities of carp in the rice-fish co-culture system[J]. Fishes, 2024, 9(7):244.

[29]
刘文舒, 郭小泽, 陈彦良, 等. 养殖黑斑蛙肠道微生物结构与功能分析[J]. 经济动物学报, 2021, 25(2):68-76.

LIU W S, GUO X Z, CHEN Y L, et al. Analysis of microbial structure and function in the intestine of farmed black-spot frog[J]. Journal of Economic Animal, 2021, 25(2):68-76. (in Chinese)

[30]
YUKGEHNAISH K, KUMAR P, SIVACHANDRAN P, et al. Gut microbiota metagenomics in aquaculture:factors influencing gut microbiome and its physiological role in fish[J]. Reviews in Aquaculture, 2020, 12(3):1903-1927.

[31]
马明星. 不同养殖密度与模式下许氏平鲉肠道菌群多样性研究[D]. 硕士学位论文. 大连: 大连海洋大学, 2023.

MA M X. Study on the diversity of the intestinal flora of Sebastodes schlegeli under different culture densities and patterns[D]. Master’s Thesis. Dalian: Dalian Ocean University, 2023. (in Chinese)

[32]
李倩, 孙丽慧, 姜建湖, 等. 放养密度对IPRA养殖太湖鲂鲌生长、抗氧化酶及肠道微生物群落的影响[J]. 水生生物学报, 2023, 47(3):479-487.

LI Q, SUN L H, JIANG J H, et al. Stocking densities on growth,antioxidant enzyme activities and intestinal microbiota of hybrid of Culter alburnus (♀)×Megalobrama terminalis () in IPRA system[J]. Acta Hydrobiologica Sinica, 2023, 47(3):479-487. (in Chinese)

[33]
邱楚雯, 施永海, 王韩信. 暗纹东方鲀不同养殖模式下的微生物群落结构[J]. 水产学报, 2021, 45(2):209-220.

QIU C W, SHI Y H, WANG H X. Microbial community structure in different cultural patterns of Takifugu obscures[J]. Journal of Fisheries of China, 2021, 45(2):209-220. (in Chinese)

[34]
WANG Y W, ZHU J, GE X, et al. Effects of stocking density on the growth performance,digestive enzyme activities,antioxidant resistance,and intestinal microflora of blunt snout bream (Megalobrama amblycephala) juveniles[J]. Aquaculture Research, 2019, 50(1):236-246.

[35]
SHIN N R, LEE J C, LEE H Y, et al. An increase in the Akkermansia spp.population induced by metformin treatment improves glucose homeostasis in diet-induced obese mice[J]. Gut, 2014, 63(5):727-735.

[36]
袁航, 胡乃捷, 陈俭, 等. 养殖密度对凡纳滨对虾生长性能及其肠道消化酶和菌群结构的影响[J]. 南方农业学报, 2023, 54(1):289-302.

YUAN H, HU N J, CHEN J, et al. Effects of stocking density on the growth performance,intestinal digestive enzyme activities and microflora structure of Litopenaeus vannamei[J]. Journal of Southern Agriculture, 2023, 54(1):289-302. (in Chinese)

[37]
DUAN Y F, CHEN H P, WANG J L, et al. Response signatures of Litopenaeus vannamei to natural Enterocytozoon hepatopenaei infection revealed by the integration of the microbiome and transcriptome[J]. Aquaculture, 2021, 542:736885.

文章导航

/