研究论文

肠道损伤对断奶仔猪生长性能、血清和空肠炎症因子影响的Meta分析

  • 陈少珍 , 1, 2 ,
  • 高靖春 2, 3, * ,
  • 姚康 2 ,
  • 蒋宗勇 2 ,
  • 曹舒婷 , 2, ** ,
  • 王丽 , 2, **
展开
  • 1 华南农业大学动物科学学院,广州 510642
  • 2 广东省农业科学院动物科学研究所,农业农村部华南动物营养与饲料重点实验室,猪禽种业全国重点实验室,广东省畜禽育种与营养重点实验室,广州 510640
  • 3 西南大学动物科学技术学院,重庆 400700
** 曹舒婷,副研究员,硕士生导师,E-mail: ;
王 丽,研究员,硕士生导师,E-mail:

* 同等贡献作者

陈少珍(1997—),女,广东清远人,硕士研究生,研究方向为猪营养与饲料。E-mail:

Copy editor: 陈鑫

收稿日期: 2024-09-20

  网络出版日期: 2025-04-15

基金资助

国家自然科学基金(U24A20447)

国家自然科学基金(32172777)

国家自然科学基金(32202730)

广东省基础与应用基础研究基金(2022A1515011406)

广东省基础与应用基础研究基金(2021A1515110636)

国家生猪产业技术体系(CARS-35)

广东省乡村振兴战略专项资金(2023TS-3-1)

A Meta-Analysis of Effects of Intestinal Injury on Growth Performance, Serum and Jejunal Inflammatory Factors in Weaned Piglets

  • CHEN Shaozhen , 1, 2 ,
  • GAO Jingchun 2, 3, * ,
  • YAO Kang 2 ,
  • JIANG Zongyong 2 ,
  • CAO Shuting , 2, ** ,
  • WANG Li , 2, **
Expand
  • 1 College of Animal Science, South China Agricultural University, Guangzhou 510642, China
  • 2 Guangdong Provincial Key Laboratory of Livestock and Poultry Breeding and Nutrition, State Key Laboratory of Swine and Poultry Breeding Industry, Key Laboratory of Animal Nutrition and Feed in South China, Ministry of Agriculture and Rural Affairs, Institute of Animal Science, Guangdong Academy of Agricultural Sciences, Guangzhou 510640, China
  • 3 College of Animal Science and Technology, Southwest University, Chongqing 400700, China
** CAO Shuting, associate professor, E-mail: ;
WANG Li, professor, E-mail:

* Contributed equally.

Received date: 2024-09-20

  Online published: 2025-04-15

摘要

为探究肠道损伤对断奶仔猪生长性能、血清和空肠炎症因子带来的影响,本试验对相关方面的研究进行了Meta分析。通过计算机对PubMed、Science Direct和Web of Science数据库进行检索,检索肠道损伤对断奶仔猪生长性能、血清和空肠炎症因子影响的随机对照试验。检索年限从2000年1月至2023年4月,设定样本纳入及排除标准进行文献筛选、数据提取,纳入总样本34篇,用Review Manager 5.4对纳入文献进行相关分析,效应指标选择标准化均数差(SMD)。结果显示: 肠道损伤能够显著降低断奶仔猪平均日增重[SMD=-1.43,95%置信区间(CI)=(-1.71,-1.15),P<0.000 1],降低平均日采食量[SMD=-1.08,95%CI=(-1.47,-0.69),P<0.000 1],提高料重比[SMD=1.06,95%CI=(0.50,1.62),P=0.000 2];肠道损伤显著提高空肠中白细胞介素-1β(IL-1β)[SMD=1.36,95%CI=(0.52,2.20),P=0.001]、肿瘤坏死因子-α(TNF-α)[SMD=0.76,95%CI=(0.22,1.30),P=0.006]、白细胞介素-6(IL-6)[SMD=0.79,95%CI=(0.26,1.32),P=0.004]以及血清中TNF-α [SMD=2.69,95%CI=(1.56,3.81),P<0.000 1]的含量。这些结果表明,肠道损伤影响断奶仔猪的生长性能,损害免疫功能。

本文引用格式

陈少珍 , 高靖春 , 姚康 , 蒋宗勇 , 曹舒婷 , 王丽 . 肠道损伤对断奶仔猪生长性能、血清和空肠炎症因子影响的Meta分析[J]. 动物营养学报, 2025 , 37(4) : 2697 -2715 . DOI: 10.12418/CJAN2025.226

Abstract

In this experiment, a Meta-analysis was performed to investigate aspects related to the effects of intestinal injury on growth performance, serum and jejunal inflammatory factors in weaned piglets. A computerized search of PubMed, Science Direct and Web of Science databases was performed to retrieve randomized controlled trials on the effects of intestinal injury models on growth performance, serum and jejunal inflammatory factors in weaned piglets. The retrieval period was from January 2000-April 2023, and the sample inclusion and exclusion criteria were set for literature screening and data extraction, and a total sample of 34 papers was included. Correlation analyses of the included studies were performed with Review Manager 5.4, and standardized mean difference (SMD) was selected for the effect indicator. The Meta-analysis showed that intestinal injury significantly reduced the average daily gain of weaned piglets [SMD=-1.43, 95% confidence interval (CI)= (-1.71, -1.15), P<0.000 1], affected average daily feed intake [SMD=-1.08, 95%CI= (-1.47, -0.69), P<0.000 1], and increased feed/gain [SMD=1.06, 95%CI= (0.50,1.62), P=0.000 2]. Moreover, intestinal injury models significantly increased jejunal interleukin-1β (IL-1β) [SMD=1.36, 95%CI= (0.52,2.20), P=0.001], tumor necrosis factor-alpha (TNF-α) [SMD=0.76, 95%CI= (0.22,1.30), P=0.006], and interleukin-6 (IL-6) contents [SMD=0.79, 95%CI= (0.26,1.32), P=0.004] and serum TNF-α content [SMD=2.69, 95%CI= (1.56,3.81), P<0.000 1]. These results suggest that intestinal injury models affect growth performance and impairs immune function in weaned piglets.

随着生猪养殖业的不断发展,现代集约化养殖体系通常采用提前断奶技术来提高母猪的生产性能,以此增加母猪的年产仔数,提高养殖设备的利用率,为养殖企业带来更多的经济效益[1-2]。断奶后,由于营养来源、生活环境、饲养管理方式发生改变,并与母猪分离和器官发育不完全等,导致仔猪胃肠道发生巨大变化,引起肠道炎症、营养物质消化吸收紊乱[3]c。早期断奶仔猪易受病原侵袭而引起腹泻,进而刺激肠黏膜分泌炎症因子并损害肠黏膜屏障的功能[4-6]。其中产肠毒素性大肠杆菌(enterotoxigenic Escherichia coli,ETEC)是引起断奶仔猪腹泻的重要病原菌[7-9]。脂多糖(lipopolysaccharide,LPS)是由脂质和多糖构成的物质,是诱导产生促炎细胞因子的关键分子[10]。LPS通过激活炎症信号通路,诱导促炎因子的关键蛋白表达,从而导致肠道屏障损伤[11]。赭曲霉毒素A(ochratoxin A,OTA)是一种分布广泛的真菌毒素,由多种曲霉属和青霉属真菌产生。OTA广泛存在于各种谷物及其副产品中,且具有多种毒性,包括肝毒性、肾毒性、肠毒性和免疫毒性等,对人类和动物健康具有很大威胁。呕吐毒素主体成分为脱氧雪腐镰刀菌烯醇(deoxynivalenol,DON),属于单端孢霉烯族化合物,主要由雪腐镰刀菌、禾谷镰刀菌、粉红镰刀菌、尖孢镰刀菌、拟枝孢镰刀菌、串珠镰刀菌等产生,存在于各种谷物及其副产品中[12-14]。DON具有多种毒性,其中以肠毒性和免疫毒性最为重要。敌草快是一种非选择性触杀性除草剂,可以利用分子氧生成超氧阴离子自由基,超氧阴离子自由基被广泛认为是诱导氧化应激的有效化学试剂。胃肠道是敌草快中毒的主要靶器官之一,消化道症状是其最早期、最突出的临床表现。敌草快进入机体后,会刺激胃肠道黏膜,导致胃肠道出血,破坏肠屏障功能。研究发现,敌草快中毒大鼠在染毒早期即可出现肠道黏膜缺血、萎缩、绒毛变短、脱落等现象[15]。Cao等[16]研究发现,敌草快诱导的氧化应激可使仔猪肠道线粒体内活性氧大量增加,损害线粒体功能并降低空肠黏膜紧密连接蛋白的丰度和上皮细胞活性,导致肠上皮完整性受损,进而增加肠道通透性。因此,常通过ETEC、LPS、DON、OTA以及敌草快等外源刺激来构建断奶仔猪肠道损伤模型,而正确认识断奶应激对肠道健康的影响,对断奶应激所导致的肠道损伤的营养调控具有重要的指导意义。
炎症细胞因子是指参与炎症反应的各种细胞因子,用于诱导T细胞活化增殖、分化等。在众多炎症细胞因子中,研究表明在肠道损伤修复中起主要作用的是肿瘤坏死因子-α(tumor necrosis factor-α, TNF-α)、白细胞介素-1β(interleukin-1β,IL-1β)、白细胞介素-6(interleukin-6,IL-6)等。TNF-α是炎症反应过程中出现最早、最重要的炎性介质,是调控机体免疫和炎症反应的重要细胞因子,能激活中性粒细胞和淋巴细胞,使血管内皮细胞通透性增加,调节其他组织代谢活性并促使其他细胞因子的合成和释放。IL-1β是一种关键的促炎细胞因子,参与多种自身免疫性炎症反应和多种细胞活动,包括细胞增殖、分化和凋亡。IL-6能诱导B细胞分化和产生抗体,并诱导T细胞活化增殖、分化,参与机体的免疫应答,是炎性反应的促发剂。
Meta分析是用于比较和综合针对同一科学问题研究结果的统计学方法。与传统综述撰写相比,它通过检索整合所有相关研究,将多个研究结果数据进行系统性的收集、评估和定量分析,给效应指标提供更精确的估计以及更加科学的结论,为增加更大的样本量提供了更精确的估计可靠性,更加全面精准,有利于探索各研究证据的一致性及研究间的差异性[17]。当多个研究结果不一致或都无统计学意义时,采用Meta分析能够得到更具统计学意义的结论。然而,各肠道损伤模型对断奶仔猪生长性能、空肠和血清炎症因子影响相关研究结果间存在差异,而对其进行Meta分析的研究较少。因此,本研究拟利用Meta分析的方法来探究肠道损伤对断奶仔猪生长性能及炎症因子的影响,为促进养猪业可持续发展提供科学支持。

1 材料与方法

1.1 检索策略

检索PubMed、Science Direct和Web of Science等数据库的相关文献,检索年限为2000年1月至2023年4月。按照表1所列的数据库和检索词对关键词进行多种排列组合方式后检索,尽可能收集更多的相关研究性文章。
表1 检索策略

Table 1 Search strategy

数据库Databases 检索词Search term
PubMed weaned piglets、intestine、LPS、ETEC、stress(应激)
Science Direct
Web of Science

1.2 文献纳入标准

纳入标准:1)研究主题是肠道损伤对断奶仔猪生长性能及免疫指标影响的相关研究;2)健康的断奶仔猪作为研究对象;3)随机对照试验,同时存在对照组和肠道损伤模型组的研究;4)结果指标设置为生长性能和炎症因子(TNF-α、IL-1β以及IL-6)。最终纳入的文献中必须具备试验组和对照组的样本量、各指标的平均值以及各指标的标准误或者标准差。

1.3 文献排除标准

排除标准:1)非试验性文章(摘要、信函、社论、专家意见、评论、案例报告、综述以及会议文章等)、重复发表以及使用同次试验数据的研究文献;2)没有空白对照组的研究文献;3)数据不足或明显有误等较低质量以及不符合纳入标准的研究文献。

1.4 数据提取

进行全文仔细阅读后,从相关的文献中提取出数据材料用于后续分析:第一作者和发表年份;研究对象及其品种;对照组和试验组的样本数;试验周期;肠道损伤的干预类型、处理途径及处理时需要添加的剂量(当纳入的研究文献中存在多种添加剂量时,先合并其数据后开展敏感性分析)。文献中出现数据不足等问题,通过发送邮件或打电话等方式联系作者,获取不足的数据进行补充[18]

1.5 统计方法

采用Review Manager 5.4标准统计程序对收集的相关数据进行统计、分析和绘制相关结果的图表[19]。在不同的研究文献中存在研究周期、研究指标及其测量单位和检测方法等方面的差异,因此最后设定本研究的效应指标为标准化均数差(standard mean difference,SMD)[19-20]。亚组分析是指在研究中,按照研究对象的某种特征(如性别、疾病严重程度等)将研究对象分成不同的亚组,然后分别估计不同组别的效应值,并进行亚组间比较,其目的在于研究交互作用或效应修饰作用,即在不同人群或条件下,效应值的大小是否不同。在本研究中,把断奶仔猪肠道损伤以及初始体重对断奶仔猪生长性能的影响分成亚组进行分析。
置信区间(confidence interval,CI)是指由样本统计量所构造的总体参数的估计区间。在统计学中,一个概率样本的CI是对这个样本的某个总体参数的区间估计。置信水平为95%的意思是多次抽样中有95%的CI包含未知的参数值而另外的5%则不包含真值。当各效应量存在于0值为无效值的95% CI上,经过统计分析得到的结果的95%CI越过0值时,说明这个研究没有办法作出一个定性结论结果分析[19-20]。结合同质性检验(检验标准为α=0.1),并使用P值和I2值对研究间的异质性进行评估:一般认为I2在0~25%为无异质性,25%~50%为轻度异质性,50%~75%为中度异质性,75%~100%为重度异质性[21]。当P<0.10时,表明研究异质性显著,则进行亚组分析。当推荐标准(40%)小于I2值时,则选取随机效应模型对本研究进行Meta分析。漏斗图是一个简单的散点图,反映研究在一定样本量或精确性下单个研究的干预效应估计值;Egger回归检验通过线性回归模型来分析效应量及其标准误差的对数值之间的关系。该模型考虑了样本大小对效应量估计的影响,特别是小样本研究可能存在的较大估计误差。发表偏倚指具有统计学显著性研究意义的研究结果较无显著性意义和无效的结果被报告和发表的可能性更大。因此,用漏斗图法和Egger线性回归法对发表偏倚进行评估。

2 结果与分析

2.1 文献检索与筛选

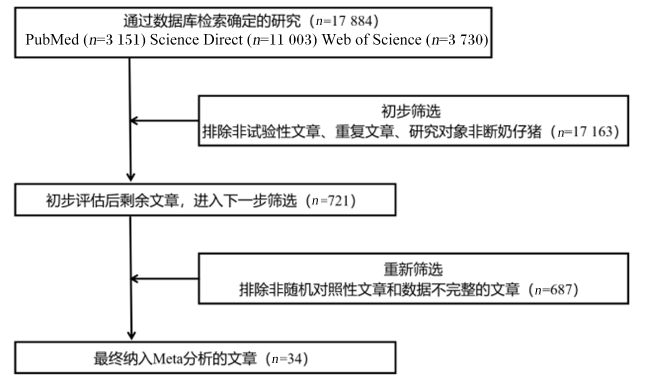
本研究根据检索策略,通过PubMed、Science Direct和Web of Science检索到的文献总共有17 884篇,通过阅读文献题目和摘要,根据文献排除标准,排除17 163篇文献,阅读全文,排除对照组不是空白组以及数据不完整的文献687篇,最终共有34篇纳入样本文献。文献筛选具体过程如图1。纳入文献基本信息见表2
图1 文献筛选流程图

Fig.1 Literature screening process

表2 文献基本信息

Table 2 Basic information of literature

序号
No.
第一作者
First
author
样本数量
Number of samples
试验
天数
Test
days/d
损伤类型
Injury type
添加量
Dosage
干预措施
Intervening measure
饲喂方式
Feeding
mode
品种
Breed
结局指标
Outcome
indicator
试验组
Test
group
对照组
Control
group
试验组
Test
group
对照组
Control
group
1 Liao等[22] 80 80 14 呕吐毒素 4 mg/kg 呕吐毒素添加 基础饲粮 饲粮添加 Duroc×Landrace×
Large Yorkshire
①②③④
2 Qiu等[23] 16 16 28 呕吐毒素 3.8 mg/kg 呕吐毒素添加 基础饲粮 饲粮添加 Duroc×(Landrace×
Yorkshire)
①②③④
3 Zha等[24] 10 10 14 呕吐毒素 4 mg/kg 呕吐毒素添加 基础饲粮 饲粮添加 Landrace×
Yorkshire
4 Zheng等[25] 6 6 25 呕吐毒素 1 097.99 μg/kg 呕吐毒素添加 基础饲粮 饲粮添加 Landrace×
Large white
5 Wang等[26] 7 7 28 呕吐毒素 4 mg/kg 呕吐毒素添加 基础饲粮 饲粮添加 Duroc×Landrace×
Large white
6 Liu等[27] 14 7 28 呕吐毒素 1 mg/kg
3 mg/kg
呕吐毒素添加 基础饲粮 饲粮添加 (Duroc×Landrace)×
Large white
7 Xiao等[28] 7 7 30 呕吐毒素 4 mg/kg 呕吐毒素添加 基础饲粮 饲粮添加 Duroc×Landrace×Large
Yorkshire
8 Zha等[24] 10 10 14 呕吐毒素 4 mg/kg 呕吐毒素添加 基础饲粮 饲粮添加 Landrace×Yorkshire
9 Jia等[29] 20 20 21 呕吐毒素 1 000.6 μg/kg 呕吐毒素添加 基础饲粮 饲粮添加 commercial Landrace-
Yorkshire crossbred
②③④
10 Yi等[30] 8 8 7 产肠毒素性
大肠杆菌
5×10⁹ CFU/mL 产肠毒素性
大肠杆菌灌服
无菌营养液 注射灌服 Duroc×Landrace×
Yorkshire
11 Pu等[31] 5 5 5 产肠毒素性
大肠杆菌
3×10¹¹ CFU/ml 产肠毒素性
大肠杆菌灌服
无菌营养液 灌服 Duroc×Landrace×
Yorkshire
①②③④
12 Li等[32] 24 24 24 h 产肠毒素性
大肠杆菌
1×10⁹ CFU/mL 产肠毒素性
大肠杆菌口服
无菌生理盐水 口服 Duroc×Landrace×
Yorkshire
②③
13 Han等[33] 30 30 14/7 产肠毒素性
大肠杆菌
1×10⁸ CFU/mL 产肠毒素性
大肠杆菌灌胃
游离培养液 灌胃 Duroc×(Landrace×
Yorkshire)
①④
14 Koo等[34] 7 7 3 产肠毒素性
大肠杆菌
6×10⁹ CFU/mL 产肠毒素性
大肠杆菌口服
口服 Duroc×(Landrace×
Yorkshire)
①②③④
15 Xu等[35] 6 6 14 产肠毒素性
大肠杆菌
1×10⁹ CFU/mL 产肠毒素性
大肠杆菌口服
无菌生理盐水 口服 Duroc×Landrace×
Large white
16 Xun等[36] 6 6 7 敌草快 10 mg/kg 敌草快注射 生理盐水 腹腔注射 Duroc×Landrace×
Large white
17 Xu等[37] 6 6 7 敌草快 10 mg/kg 敌草快注射 生理盐水 腹腔注射 Duroc×Landrace×
Large white
18 Cao等[16] 6 6 7 敌草快 10 mg/kg 敌草快注射 生理盐水 腹腔注射 Duroc×Landrace×
Large white
19 Yuan等[38] 32 32 7 敌草快 8 mg/kg 敌草快注射 生理盐水 腹腔注射 Duroc×Landrace×
Large white
①②③④
20 Qiu等[39] 21 7 35 草甘膦 0、10、20、40 mg/kg 草甘膦添加 基础饲粮 饲粮添加 Duroc×Landrace×
Large white
②③④
21 Zhang等[40] 24 12 42 赭曲霉毒素A 4 mg/kg
8 mg/kg
赭曲霉毒素A添加 基础饲粮 饲粮添加 Duroc×(Landrace×
Yorkshire)
22 Xue等[41] 12 12 7 脂多糖 100 μg/kg 脂多糖注射 生理盐水 腹腔注射 Duroc×Landrace×
Large
23 Zhang等[42] 6 6 14 脂多糖 100 μg/kg 脂多糖注射 生理盐水 腹腔注射 Duroc×Landrace×
Yorkshire
24 Huang等[43] 10 10 7 脂多糖 60~80 μg/kg 脂多糖注射 生理盐水 腹腔注射 Duroc×Landrace×
Yorkshire
①②③④
25 Hou等[44] 6 6 6 脂多糖 80 μg/kg 脂多糖注射 生理盐水 腹腔注射 Duroc×Landrace×
Yorkshire
26 Chen等[45] 6 6 4 h 脂多糖 100 μg/kg 脂多糖注射 生理盐水 腹腔注射 Duroc×Landrace×
Large white
27 Xiao等[46] 6 6 4 h 脂多糖 100 μg/kg 脂多糖注射 生理盐水 腹腔注射 Duroc×Landrace×
Yorkshire
②③④
28 Wang等[47] 6 6 4 h 脂多糖 100 μg/kg 脂多糖注射 生理盐水 腹腔注射 Duroc×Large white×
Landrace
29 Waititu等[48] 6 6 5 d/6 h 脂多糖 60 μg/kg 脂多糖注射 生理盐水 肌肉注射 Duroc×(Yorkshire×
Landrace)
①②
30 Jiao等[49] 6 6 4 h 脂多糖 100 μg/kg 脂多糖注射 生理盐水 腹腔注射 Duroc×Landrace×
Yorkshire
②③④
31 Zhu等[50] 12 12 7 脂多糖 200 μg/kg 脂多糖注射 生理盐水 腹腔注射 Duroc×(Landrace×
Large white)
32 Fan等[51] 12 12 7 脂多糖 100 μg/kg 脂多糖 生理盐水 腹腔内灌胃 Duroc×Large
White×Landrace
①②③
33 Ahasan等[52] 12 12 10 脂多糖 67.2~84.3 μg/kg 脂多糖注射 生理盐水 肌肉注射 Topigs 40×Topdelta
34 Mao等[53] 18 18 7/3 h 脂多糖 200 μg/kg 脂多糖注射 生理盐水 肌肉注射 Large white×Landrace
×Pietran

①:生长性能(平均日增重、平均日采食量、料重比) growth performance (ADG, ADFI, F/G);②:肿瘤坏死因子-α:tumor necrosis factor-α;③:白细胞介素-6 interleukin-6;④:白细胞介素-1β interleukin-1β。

2.2 肠道损伤对断奶仔猪生长性能影响的森林图、敏感性分析及漏斗图

2.2.1 肠道损伤对断奶仔猪平均日增重(ADG)的影响
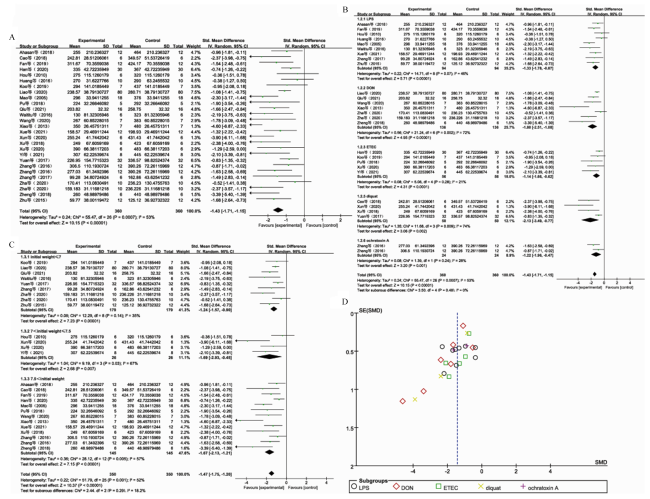
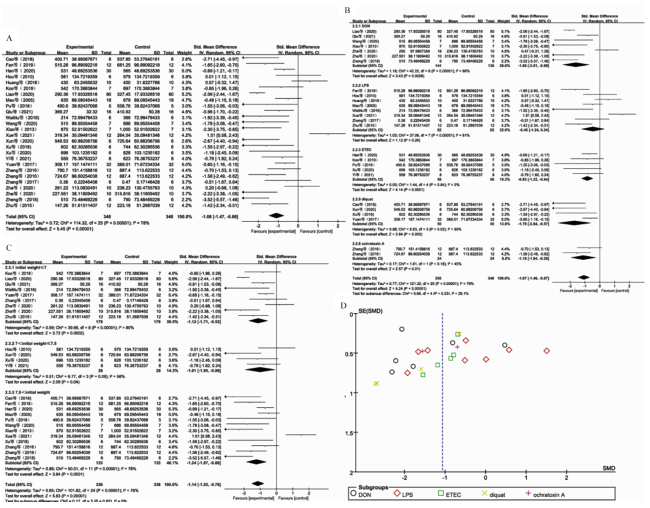
在最终纳入样本文献34篇中,报道了断奶仔猪肠道损伤与ADG之间的关系的研究共有26项。结果表明,纳入的研究间存在异质性(df=26;I2=53%;P<0.000 1),因此选择随机效应模型对效应值进行Meta分析。如图2-A所示,肠道损伤与断奶仔猪ADG间具有统计学相关性[SMD=-1.43,95%CI为(-1.71,-1.15)]。由于异质性较大(I2=53%),根据纳入文献中损伤模型的类型进行分类(LPS模型组、DON模型组、ETEC模型组、敌草快模型组以及OTA模型组),并作出亚组分析,结果表明,OTA模型组(I2=28%)和LPS模型组(I2=46%)与ADG间存在轻度异质性,DON模型组(I2=72%)和敌草快模型组(I2=74%)存在中度异质性(图2-B)。
图2 肠道损伤对断奶仔猪平均日增重影响的结果图

A:平均日增重的森林图;B:平均日增重的亚组分析图(损伤模型亚组);C:平均日增重的亚组分析图(断奶仔猪初重亚组);D:平均日增重的漏斗图。A:forest plot of average daily gain;B:subgroup analysis plot of average daily gain (injury model subgroup);C:subgroup analysis plot of average daily gain (weaned piglet initial weight subgroup);D:funnel plot of average daily gain.

Experimental:试验组 experimental group;Control:对照组 control group;Std.Mean Difference:标准化均数差standardized mean difference;Study or Subgroup:研究或组别;Mean:均值;SD:标准差standard deviation;Total:样本数 sample number;Weight:权重;95% CI:95%置信区间95% confidence interval;Heterogeneity:异质性;df:自由度 degree of freedom;I2:异质性检验 heterogeneity test;Test for overall effect:总体效应检验;Favours(control):对照组获益;Favours(experimental):试验组获益;Test for subaroub differences:亚组差异;LPS:脂多糖模型组 lipopolysaccharide model group;DON:呕吐毒素模型组deoxynivalenol model group;ETEC:产肠毒素性大肠杆菌模型组enterotoxigenic Escherichia coli model group;diquat:敌草快模型组 diquat model group;ochratoxin A:赭曲霉毒素A模型组(OTA模型组)ochratoxin A model group (OTA model group); SE(SMD):标准化均数差 standardized mean difference;Subgroups:亚组。下图同 the same as below。

Fig.2 Result plot of effects of intestinal damage on average daily gain of weaned piglets

以上结果表明,肠道损伤的模型均显著降低断奶仔猪ADG(图2-B)。为了研究断奶仔猪的初始体重对肠道损伤的ADG的影响,根据纳入的相关文献,依据断奶仔猪的初始体重进行分类与亚组分析(①initial weight≤7 kg;②7 kg<initial weight≤7.5 kg;③initial weight>7.5 kg)。结果表明,断奶仔猪的初始体重对肠道损伤造成的ADG变化没有影响(图2-C)。最后,采用Egger线性回归法及漏斗图法检验发表偏倚,其P=0.001,表明ADG存在发表偏倚(图2-D)。综上所述,肠道损伤显著降低断奶仔猪ADG。

2.2.2 肠道损伤对断奶仔猪平均日采食量(ADFI)的影响

在最终纳入样本文献34篇中,报道了断奶仔猪肠道损伤与ADFI之间的关系的研究共有26项。由森林图可知(图3-A),纳入的研究间存在异质性(df=25;I2=78%;P<0.000 1),因此选择随机效应模型对效应值进行Meta分析。结果表明(图3-A),肠道损伤与断奶仔猪ADFI间存在统计学相关性[SMD=-1.08,95%CI为(-1.47,-0.69)]。亚组分析结果表明(图3-B),除ETEC模型组不存在异质性外(I2=0),其他因素造成断奶仔猪肠道损伤的模型均存在异质性,但LPS模型组95%CI跨越了无效值,因此,LPS模型组没有统计学意义。以上结果表明,各肠道损伤模型断奶仔猪ADFI均显著降低(图3-B)。进一步探究断奶仔猪的初始体重对肠道损伤的ADFI的影响,根据纳入的相关文献,将断奶仔猪按照初始体重(①initial weight≤7 kg;②7 kg<initial weight≤7.5 kg;③initial weight>7.5 kg)进行分类与亚组分析。结果表明(图3-C),断奶仔猪的初始体重对肠道损伤造成的ADFI的变化没有显著影响。最后,采用Egger线性回归法及漏斗图法检验发表偏倚,结果发现其P=0.614,表明不存在发表偏倚(图3-D)。最终结果表明,断奶仔猪ADFI与肠道损伤模型之间具有统计学的相关性,而且肠道损伤显著降低断奶仔猪ADFI。
图3 肠道损伤对断奶仔猪平均日采食量影响的结果图

A:平均日采食量的森林图;B:平均日采食量的亚组分析图(损伤模型亚组);C:平均日采食量的亚组分析图(断奶仔猪初重亚组);D:平均日采食量的漏斗图。A:forest plot of average daily feed intake;B:subgroup analysis plot of average daily feed intake (injury model subgroup);C:subgroup analysis plot of average daily feed intake (weaned piglet initial weight subgroup);D:funnel plot of average daily feed intake.

Fig.3 Result plot of effects of intestinal damage on average daily feed intake of weaned piglets

2.2.3 肠道损伤对断奶仔猪料重比(F/G)的影响

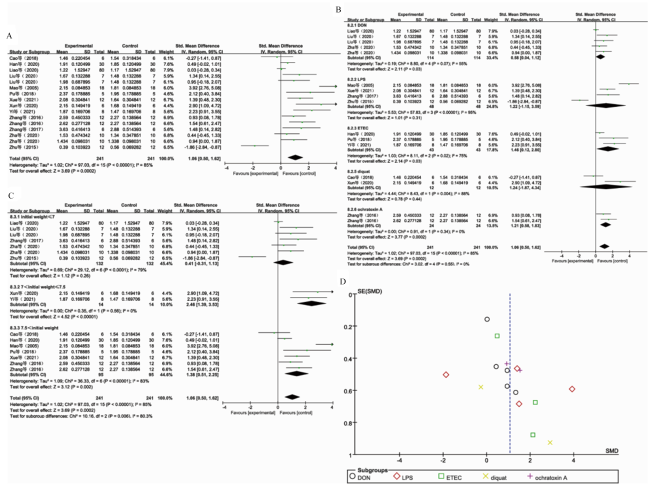
在最终纳入样本文献34篇中,报道了断奶仔猪肠道损伤与F/G之间的关系的研究共有16项。分析结果显示(图4-A),纳入的研究间存在异质性(df=15;I2=85%;P=0.000 2),因此选择随机效应模型对效应值进行Meta分析。结果表明(图4-A),肠道损伤与断奶仔猪F/G间具有统计学相关性[SMD=1.06,95%CI为(0.50,1.62)]。亚组分析的结果表明(图4-B),OTA模型组不存在异质性(I2=0),ETEC模型组存在重度异质性(I2=75%),而DON模型组、敌草快模型组和LPS模型组的95%CI均跨越了无效值,因此无统计学意义。以上结果表明,各肠道损伤模型均显著提高断奶仔猪F/G(图4-B)。为了研究断奶仔猪的初始体重对肠道损伤F/G的影响,根据纳入的相关文献,根据断奶仔猪初始体重进行分类与亚组分析(①initial weight≤7 kg;②7 kg<initial weight≤7.5 kg;③initial weight>7.5 kg)。结果表明(图4-C),断奶仔猪的初始体重在大于7 kg对肠道损伤造成的F/G的变化没有显著影响。最后,采用漏斗图法检验发表偏倚,结果发现其P=0.053,说明不存在发表偏倚(图4-D)。最终结果表明,肠道损伤显著提高断奶仔猪F/G。
图4 肠道损伤对断奶仔猪料重比影响的结果图

A:料重比的森林图;B:料重比的亚组分析图(损伤模型亚组);C:料重比的亚组分析图(断奶仔猪初重亚组);D:料重比的漏斗图。A:forest plot of feed/gain;B:subgroup analysis plot of feed/gain (injury model subgroup);C:subgroup analysis plot of feed/gain (weaned piglet initial weight subgroup);D:funnel plot of feed/gain.

Fig.4 Result plot of effects of intestinal damage on feed/gain of weaned piglets

2.3 肠道损伤对断奶仔猪血清和空肠炎症因子影响的森林图、敏感性分析及漏斗图

2.3.1 肠道损伤对断奶仔猪空肠IL-1β含量的影响
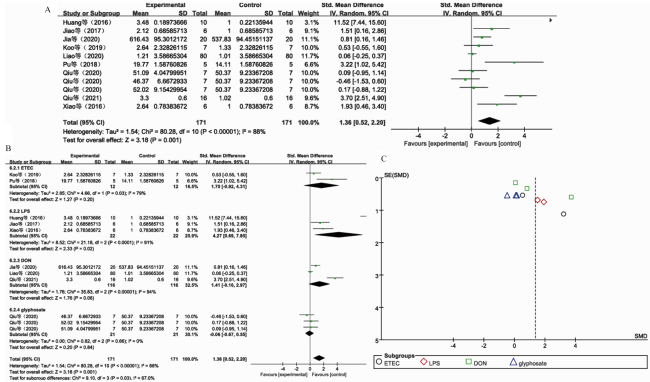
在最终纳入样本文献34篇中,报道了肠道损伤与断奶仔猪空肠IL-1β含量之间的关系的研究共有11项。从森林图可以看出(图5-A),断奶仔猪空肠中IL-1β含量在肠道损伤仔猪中具有统计学相关性,且具有重度异质性[SMD=1.36,95%CI为(0.52,2.20);df=10;I2=88%;P=0.001]。亚组分析的结果表明(图5-B),ETEC模型组(I2=79%)、LPS模型组(I2=91%)以及DON模型组(I2=94%)具有重度异质性,草甘膦模型组95%CI值均跨越无效值,因此无统计学意义。以上结果表明,各肠道损伤模型均显著提高断奶仔猪空肠中IL-1β含量(图5-B)。最后,采用漏斗图法及Egger线性回归法检验发表偏倚,结果发现其P=0.014,该研究肠道损伤与断奶仔猪空肠IL-1β含量之间存在发表偏倚(图5-C)。
图5 肠道损伤对断奶仔猪空肠IL-1β含量影响的结果图

A:空肠IL-1β含量的森林图;B:空肠IL-1β含量的亚组分析图;C:空肠IL-1β含量的漏斗图。A:forest plot of jejunal IL-1β content;B:subgroup analysis plot of jejunal IL-1β content;C:funnel plot of jejunal IL-1β content.

glyphosate:草甘膦模型组 glyphosate model group。

Fig.5 Result plot of effects of intestinal injury on jejunal IL-1β content of weaned piglet

2.3.2 肠道损伤对断奶仔猪空肠TNF-α含量影响

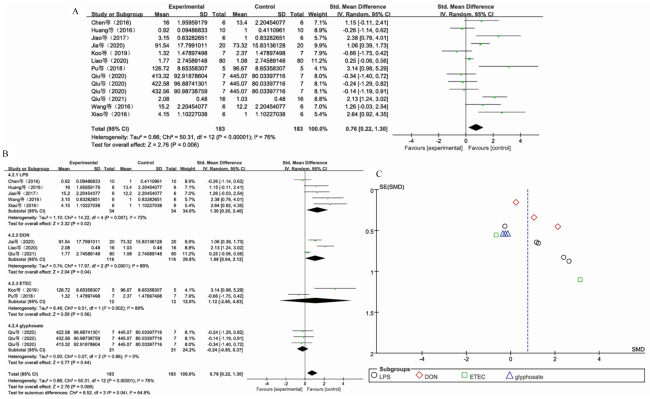
在最终纳入样本文献34篇中,报道了肠道损伤与断奶仔猪空肠TNF-α含量之间的关系的研究共有13项。从森林图中可以看出(图6-A),断奶仔猪空肠中TNF-α的含量在肠道损伤仔猪中具有统计学相关性,且存在重度异质性[SMD=0.76,95%CI为(0.22,1.30);df=12;I2=76%;P=0.006]。亚组分析的结果表明(图6-B),LPS模型组(I2=72%)具有中度异质性,DON模型组(I2=89%)和ETEC模型组(I2=89%)具有重度异质性,草甘膦模型组95%CI值均跨越无效值,因此无统计学意义。以上结果表明,各肠道损伤模型均显著提高断奶仔猪空肠中TNF-α含量(图6-B)。最后,采用漏斗图法及Egger线性回归法检验发表偏倚,结果发现其P=0.148,表示该Meta分析不存在发表偏倚(图6-C)。
图6 肠道损伤对断奶仔猪空肠TNF-α含量影响的结果图

A:空肠TNF-α含量的森林图;B:空肠TNF-α含量的亚组分析图;C:空肠TNF-α含量的漏斗图。A:forest plot of jejunal TNF-α contet;B:subgroup analysis plot of jejunal TNF-α content;C:funnel plot of jejunal TNF-α content.

glyphosate:草甘膦模型组 glyphosate model group。

Fig.6 Result plot of effects of intestinal injury on jejunal TNF-α content of weaned piglets

2.3.3 肠道损伤对断奶仔猪血清中TNF-α含量的影响

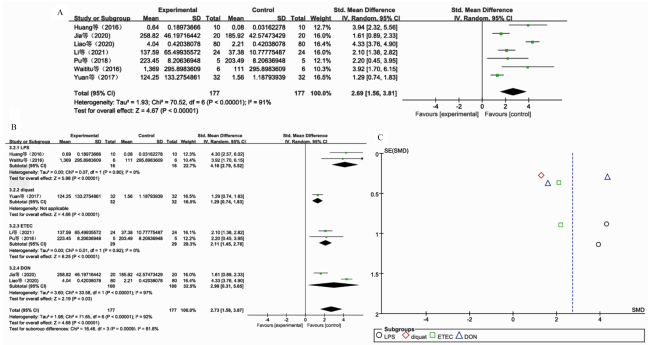
同时,本试验还对断奶仔猪血清中的TNF-α含量进行了Meta分析。在最终纳入样本文献34篇中,报道了肠道损伤与断奶仔猪血清TNF-α含量之间的关系的研究共有7项。结果发现(图7-A),断奶仔猪血清中TNF-α的含量在肠道损伤仔猪中具有统计学相关性,且存在重度异质性[SMD=2.69,95%CI为(1.56,3.81);df=6;I2=91%;P<0.000 1]。亚组分析结果表明(图7-B),DON模型组具有重度异质性(I2=97%),LPS模型组和ETEC模型组均不存在异质性(I2均为0),然而,由于缺乏有关敌草快仔猪肠道损伤模型的文献,未能显示出异质性。以上结果表明,各肠道损伤模型均显著提高血清中TNF-α的含量(图7-B)。采用漏斗图法及Egger线性回归法检验发表偏倚,结果发现其P=0.671,表示不存在发表偏倚(图7-C)。
图7 肠道损伤对断奶仔猪血清TNF-α影响的结果图

A:血清TNF-α含量的森林图;B:血清TNF-α含量的亚组分析图;C:血清TNF-α含量的漏斗图。

Fig.7 Result plot of effects of intestinal injury on serum TNF-α content of weaned piglets

A:forest plot of serum TNF-α content;B:subgroup analysis plot of serum TNF-α content;C:funnel plot of serum TNF-α content.

2.3.4 肠道损伤对断奶仔猪空肠中IL-6含量的影响

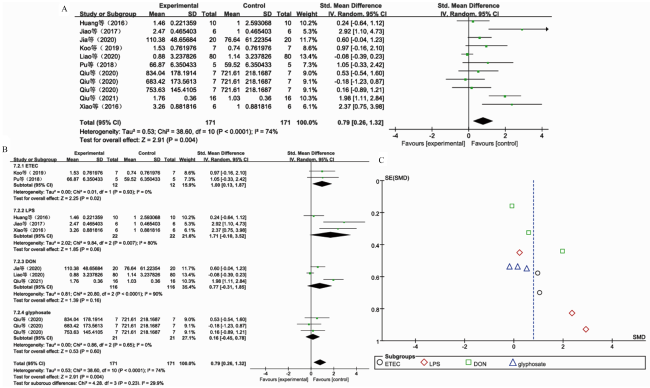
在最终纳入样本文献34篇中,报道了肠道损伤与断奶仔猪空肠IL-6含量之间的关系的研究共有11项。图8-A显示,断奶仔猪空肠中IL-6的含量在肠道损伤仔猪中存在统计学相关性,且存在中度异质性[SMD=0.79,95%CI为(0.26,1.32);df=10;I2=74%;P=0.004]。通过亚组分析结果表明(图8-B),DON模型组、草甘膦模型组和LPS模型组95%CI值跨越无效值,因此无统计学意义。以上结果表明,各肠道损伤模型均显著提高空肠中IL-6的含量(图8-B)。采用漏斗图法及Egger线性回归法检验发表偏倚,结果发现其P=0.013,表示该Meta分析存在发表偏倚(图8-C)。
图8 肠道损伤对断奶仔猪空肠IL-6含量影响的结果图

A:空肠IL-6含量的森林图;B:空肠IL-6含量的亚组分析图;C:空肠IL-6含量的漏斗图。A:forest plot of jejunal IL-6 content;B:subgroup analysis plot of jejunal IL-6 conent;C:funnel plot of jejunal IL-6 content.

glyphosate:草甘膦模型组 glyphosate model group。

Fig.8 Result plot of effects of intestinal injury on jejunal IL-6 content of weaned piglets

3 讨论

随着现代集约化养猪模式的不断扩张,由致病性大肠杆菌引发的仔猪腹泻问题日益凸显,已成为导致仔猪高死亡率的关键因素之一。其中,仔猪黄痢、仔猪白痢及水肿病作为该病原体的三大常见病症,对养猪业构成了严峻的挑战,不仅造成了巨大的经济损失,还严重阻碍了猪养殖业的可持续发展进程[54]。ETEC是仔猪大肠杆菌病最重要的病变型,新生仔猪和断奶仔猪ETEC感染后导致的腹泻在仔猪群体中广泛传播,常常会波及整个猪群,并呈现出周期性发生的特点,严重影响了仔猪的健康状况,还导致防控成本大幅度升高[55]。LPS是一种内毒素,是革兰氏阴性细菌外膜的关键致病成分,可引起免疫细胞释放大量炎性细胞因子,引发肠道屏障受损、肠道炎症和肠道形态受损,最终降低仔猪生长性能。霉菌毒素是真菌产生的次级代谢产物,食品和饲料储存保管不当,极易发生霉菌毒素污染,猪采食霉菌毒素污染的饲粮后,会出现呕吐、腹泻、免疫力降低、生长发育受阻等不良现象[56]。其中OTA是曲霉菌属和青菌属中多种丝状真菌的二级代谢产物[57-58],会影响宿主的肠道屏障和吸收功能,具有肠道毒性[59-60]。此外,OTA能够增加其他病原体对动物肠道造成的损伤外,OTA还能够影响机体的免疫功能,导致主要免疫器官体积缩小(脑、脾脏等),抑制抗体反应,影响免疫细胞的增殖及功能受损等[61-62]。而DON是食品和饲料中常见的真菌毒素,肠道是DON的主要吸收部位,并成为这种毒素的主要靶点,呕吐毒素被猪摄入后,可以通过改变微生物区系组成,降低黏蛋白、紧密连接蛋白的表达水平以及调控免疫因子,破坏肠道的生物屏障、化学屏障、物理屏障和免疫屏障,对猪机体造成严重的危害[63]。因此,DON在动物体内表现出明显的肠毒性。有研究表明,饲粮被DON(1~2 mg/kg)污染84 d后,被仔猪食用,显著下调了仔猪回肠中的炎症因子白细胞介素-8(IL-8)、IL-1β表达水平[64]。因此,常通过ETEC、LPS、OTA、DON等外源刺激来构建断奶仔猪肠道损伤模型,以此肠道损伤模型来对断奶仔猪生长性能、血清和空肠炎症因子的影响进行Meta分析。
仔猪的生长性能与其健康状况密切相关,断奶应激的仔猪通常表现出较差的生长性能[65]。研究表明,断奶仔猪初始体重大小可能会影响后期生长性能。Cao等[66]研究表明,断奶后第1周的生长性能显著降低,直到第3周才恢复到哺乳仔猪的水平。在本研究中发现,各因素造成的肠道损伤均显著降低断奶仔猪ADG,影响ADFI,降低F/G。断奶仔猪的初始体重对肠道损伤造成的ADG和ADFI的变化没有显著影响,断奶仔猪的初始体重在大于7 kg对肠道损伤造成的F/G的变化没有显著影响。同时,有研究发现仔猪早期断奶会导致肠道菌群、宿主生理生化功能、肠道消化吸收能力以及黏膜免疫功能的紊乱[67-68],最终导致采食量减少,断奶后腹泻的发生和生长受限[69]
细胞因子是由多种组织细胞(主要为免疫细胞)以及一些其他非免疫细胞共同分泌的一类小分子蛋白,是免疫系统不可或缺的信息分子,在免疫调节过程中扮演非常重要的角色[70]。而白细胞介素是细胞因子组成部分之一,其功能是可以介导细胞之间的相互作用、参与炎症反应和调节免疫应答等[70]。断奶应激不仅导致肠道T淋巴细胞[71-72]和肥大细胞等免疫细胞功能障碍,而且激活肠道免疫系统产生大量促炎细胞因子(TNF-α、IFN-γ、IL-1β、IL-6、IL-8)[73-80]。肠道促炎细胞因子的过度表达会破坏肠黏膜的完整性,并且使组织通透性增加[80-81]。细胞因子的抑制可以阻止某些病原体的繁殖,这有助于肠道微生态系统的稳定性。本研究发现,肠道损伤显著提高断奶仔猪空肠中IL-1β、TNF-α、IL-6含量以及血清中TNF-α的含量。而断奶导致肠道完整性破坏,微生物入侵刺激仔猪空肠中分泌的免疫球蛋白A和防御素的表达[76],有利于断奶后肠道屏障功能的恢复。总而言之,这些结果表明肠道损伤影响断奶仔猪的免疫功能。

4 结论

本研究结果显示,肠道损伤影响断奶仔猪生长性能、免疫功能。本研究利用Meta分析对国内外相关文献的结果进行合并,从统计层面为肠道损伤对断奶仔猪生长性能及空肠、血清中炎症因子的影响给予一定的数据参考。
[1]
CAMPBELL J M, CRENSHAW J D, POLO J. The biological stress of early weaned piglets[J]. Journal of Animal Science and Biotechnology, 2013, 4(1):19.

[2]
王金语. 不同形式氧化锌对断奶仔猪生长性能、血液指标、肠道屏障的影响[D]. 硕士学位论文. 沈阳: 沈阳农业大学, 2019.

WANG J Y. Effects of different forms of zinc oxide on growth performance,blood indexes and intestinal barrier of weaned piglets[D]. Master’s Thesis. Shenyang: Shenyang Agricultural University, 2019. (in Chinese)

[3]
LI Y, GUO Y, WEN Z S, et al. Weaning stress perturbs gut microbiome and its metabolic profile in piglets[J]. Scientific Reports, 2018, 8(1):18068.

DOI PMID

[4]
LODEMANN U, AMASHEH S, RADLOFF J, et al. Effects of ex vivo infection with ETEC on jejunal barrier properties and cytokine expression in probiotic-supplemented pigs[J]. Digestive Diseases and Sciences, 2017, 62(4):922-933.

[5]
JI F J, WANG L X, YANG H S, et al. Review:the roles and functions of glutamine on intestinal health and performance of weaning pigs[J]. Animal, 2019, 13(11):2727-2735.

[6]
GRESSE R, CHAUCHEYRAS-DURAND F, FLEURY M A, et al. Gut microbiota dysbiosis in postweaning piglets:understanding the keys to health[J]. Trends in Microbiology, 2017, 25(10):851-873.

[7]
DUBREUIL J D. Pig vaccination strategies based on enterotoxigenic Escherichia coli toxins[J]. Brazilian Journal of Microbiology, 2021, 52(4):2499-2509.

[8]
周锐, 王俊, 刘文婷, 等. 产肠毒素大肠杆菌黏附素受体结合域的表达及其抗ETEC黏附效果的研究[C]// 中国畜牧兽医学会动物营养学分会第七届中国饲料营养学术研讨会. 郑州: 中国畜牧兽医学会动物营养学分会,2014:103.

ZHOU R, WANGJ, LIUW T, et al. Expression of the adhesin receptor binding domain of enterotoxin-producing Escherichia coli and its anti-ETEC adhesion effect:7th Chinese feed nutrition symposium of the animal nutrition branch of the chinese animal husbandry and veterinary medical association[C]// The 7th China Feed Nutrition Academic Symposium of the Animal Nutrition Branch of the Chinese Society of Animal Husbandry and Veterinary Medicine. Zhengzhou: Animal Nutrition Branch of the Chinese Society of Animal Husbandry and Veterinary Medicine,2014:103. (in Chinese)

[9]
高莹, 李淼, 孙元, 等. 乳酸乳球菌表达系统的发展现状与前景展望[J]. 微生物学报, 2022, 62(3):895-905.

GAO Y, LI M, SUN Y, et al. Development and prospects of Lactococcus lactis expression system[J]. Acta Microbiologica Sinica, 2022, 62(3):895-905. (in Chinese)

[10]
WILLIAMS J M, DUCKWORTH C A, CAMPBELL B J, et al. Mo1807 lipopolysaccharide induces small intestinal epithelial cell apoptosis and shedding by a TLR4 and TNFR1 dependent mechanism, which is regulated by NFκB signalling[J]. Gastroenterology, 2013, 144(5S1):668.

[11]
CIESIELSKA A, MATYJEK M, KWIATKOWSKA K. TLR4 and CD14 trafficking and its influence on LPS-induced pro-inflammatory signaling[J]. Cellular and Molecular Life Sciences, 2021, 78(4):1233-1261.

DOI PMID

[12]
巩性涛, 王培, 肖理文, 等. 呕吐毒素荧光定量快速检测试纸卡及仪器技术性能优化的研究报告[J]. 粮食加工, 2021, 46(2):84-91.

GONG X T, WANG P, XIAO L W, et al. Research report on technical performance optimization on instruction of the quantitative & rapid test strip for deoxynivalenol[J]. Grain Processing, 2021, 46(2):84-91. (in Chinese)

[13]
赵志龙, 李春晓, 牛亚飞, 等. 面粉中呕吐毒素污染及相关降解研究[J]. 现代食品, 2018(19):15-17, 25.

ZHAO Z L, LI C X, NIU Y F, et al. Study on vomiting toxin pollution and related degradation in flour[J]. Modern Food, 2018(19):15-17, 25. (in Chinese)

[14]
肖理文, 徐秀, 赵皖, 等. 基于时间分辨荧光纳米微球的呕吐毒素快速定量检测试纸条的研制及性能研究[J]. 粮食加工, 2017, 42(3):36-39.

XIAO L W, XU X, ZHAO W, et al. Development and performance study of test strips for rapid quantitative detection of vomitoxin based on time-resolved fluorescent nanorods[J]. Grain Processing, 2017, 42(3):36-39. (in Chinese)

[15]
张建爽. 敌草快中毒大鼠毒代动力学及细胞焦亡在肠道损伤中的作用机制研究[D]. 硕士学位论文. 石家庄: 河北医科大学, 2023.

ZHANG J S. Toxicokinetics of diquat poisoning in rats and the mechanism of cellular death in intestinal injury[D]. Master’s Thesis. Shijiazhuang: Hebei Medical University, 2023. (in Chinese)

[16]
CAO S T, WU H, WANG C C, et al. Diquat-induced oxidative stress increases intestinal permeability,impairs mitochondrial function,and triggers mitophagy in piglets[J]. Journal of Animal Science, 2018, 96(5):1795-1805.

[17]
SAUVANT D, SCHMIDELY P, DAUDIN J J, et al. Meta-analyses of experimental data in animal nutrition[J]. Animal, 2008, 2(8):1203-1214.

DOI PMID

[18]
高靖春, 曹舒婷, 蒋宗勇, 等. 益生菌对断奶仔猪肠道屏障功能影响的Meta分析[J]. 动物营养学报, 2022, 34(5):3317-3328.

DOI

GAO J C, CAO S T, JIANG Z Y, et al. Meta analysis of effects of probiotics on intestinal barrier function of weaned piglets[J]. Chinese Journal of Animal Nutrition, 2022, 34(5):3317-3328. (in Chinese)

DOI

[19]
高靖春, 曹舒婷, 姚康, 等. 益生菌对肠道损伤条件下断奶仔猪生长性能影响的Meta分析[J]. 动物营养学报, 2023, 35(3):1520-1531.

DOI

GAO J C, CAO S T, YAO K, et al. A Meta analysis of effects of probiotics on growth performance of weaned piglets under intestinal injury conditions[J]. Chinese Journal of Animal Nutrition, 2023, 35(3):1520-1531. (in Chinese)

DOI

[20]
苏亚北, 许欣纯, 林楚晓, 等. 益生菌对肉鸡生长性能影响的Meta分析[J]. 饲料工业, 2023, 44(10):52-60.

SU Y B, XU X C, LIN C X, et al. Meta-analysis of the effect of probiotics on the growth performance of broilers[J]. Feed Industry, 2023, 44(10):52-60. (in Chinese)

[21]
薛丽名. ALPPS与PVE两步肝切除术的Meta分析[D]. 硕士学位论文. 西宁: 青海大学, 2017.

XUE L M. A Meta-analysis of safety and efficacy of associating liver partition and portal vein ligation for staged hepatectomy (ALPPS) versus portal vein embolization after stage hepatectomy (PVE)[D]. Master’s Thesis. Xining: Qinghai University, 2017. (in Chinese)

[22]
LIAO P, LI Y H, LI M J, et al. Baicalin alleviates deoxynivalenol-induced intestinal inflammation and oxidative stress damage by inhibiting NF-κB and increasing mTOR signaling pathways in piglets[J]. Food and Chemical Toxicology, 2020,140:111326.

[23]
QIU Y Q, YANG J, WANG L, et al. Dietary resveratrol attenuation of intestinal inflammation and oxidative damage is linked to the alteration of gut microbiota and butyrate in piglets challenged with deoxynivalenol[J]. Journal of Animal Science and Biotechnology, 2021, 12(1):71.

DOI PMID

[24]
ZHA A, LIAO P, TAN B, et al. Dietary baicalin zinc supplementation alleviates oxidative stress and enhances nutrition absorption in deoxynivalenol challenged pigs[J]. Current drug metabolism, 2020,21.

[25]
ZHENG W J, JI X, ZHANG Q, et al. Hydrogen-rich water and lactulose protect against growth suppression and oxidative stress in female piglets fed fusarium toxins contaminated diets[J]. Toxins, 2018, 10(6):228.

[26]
WANG S, ZHANG C, YANG J C, et al. Sodium butyrate protects the intestinal barrier by modulating intestinal host defense peptide expression and gut microbiota after a challenge with deoxynivalenol in weaned piglets[J]. Journal of Agricultural and Food Chemistry, 2020, 68(15):4515-4527.

DOI PMID

[27]
LIU M, ZHANG L, CHU X H, et al. Effects of deoxynivalenol on the porcine growth performance and intestinal microbiota and potential remediation by a modified HSCAS binder[J]. Food and Chemical Toxicology, 2020,141:111373.

[28]
XIAO H, TAN B E, YIN Y L, et al. Effects of composite antimicrobial peptides in weanling piglets challenged with deoxynivalenol:Ⅱ.Intestinal morphology[J]. Journal of Animal Science, 2013, 91(10):4750-4756.

[29]
JIA R, LIU W B, ZHAO L H, et al. Low doses of individual and combined deoxynivalenol and zearalenone in naturally moldy diets impair intestinal functions via inducing inflammation and disrupting epithelial barrier in the intestine of piglets[J]. Toxicology Letters, 2020,333:159-169.

[30]
YI Q, LIU J, ZHANG Y, et al. Anethole attenuates enterotoxigenic Escherichia coli-induced intestinal barrier disruption and intestinal inflammation via modification of TLR signaling and intestinal microbiota[J]. Frontiers in Microbiology, 2021,12:647242.

[31]
PU J N, CHEN D W, TIAN G, et al. Protective effects of benzoic acid,Bacillus coagulans,and oregano oil on intestinal injury caused by enterotoxigenic Escherichia coli in weaned piglets[J]. BioMed Research International, 2018,2018:1829632.

[32]
LI H H, LIU X J, SHANG Z Y, et al. Clostridium butyricum helps to alleviate inflammation in weaned piglets challenged with enterotoxigenic Escherichia coli K88[J]. Frontiers in Veterinary Science, 2021,8:683863.

[33]
HAN Y, ZHAN T, ZHAO Q, et al. Effects of mixed organic acids and medium chain fatty acids as antibiotic alternatives on the performance,serum immunity,and intestinal health of weaned piglets orally challenged with Escherichia coli K88[J]. Animal Feed Science and Technology, 2020,269:114617.

[34]
KOO B, BUSTAMANTE-GARCÍA D, KIM J W, et al. Health-promoting effects of Lactobacillus-fermented barley in weaned pigs challenged with Escherichia coli K88+[J]. Animal, 2020, 14(1):39-49.

[35]
XU Y, LAHAYE L, HE Z, et al. Micro-encapsulated essential oils and organic acids combination improves intestinal barrier function,inflammatory responses and microbiota of weaned piglets challenged with enterotoxigenic Escherichia coli F4 (K88+)[J]. Animal Nutrition, 2020, 6(3):269-277.

[36]
XUN W J, FU Q Y, HOU G Y, et al. Protective effects of dietary resveratrol supplementation against oxidative stress in diquat-challenged piglets[J]. Italian Journal of Animal Science, 2020, 19(1):1523-1532.

[37]
XU Y Q, XING Y Y, WANG Z Q, et al. Pre-protective effects of dietary chitosan supplementation against oxidative stress induced by diquat in weaned piglets[J]. Cell Stress and Chaperones, 2018, 23(4):703-710.

[38]
YUAN D X, HUSSAIN T, TAN B, et al. The evaluation of antioxidant and anti-inflammatory effects of Eucommia ulmoides flavones using diquat-challenged piglet models[J]. Oxidative Medicine and Cellular Longevity, 2017,2017:8140962.

[39]
QIU S N, FU H Y, ZHOU R Y, et al. Toxic effects of glyphosate on intestinal morphology,antioxidant capacity and barrier function in weaned piglets[J]. Ecotoxicology and Environmental Safety, 2020,187:109846.

[40]
ZHANG Z Q, GAN F, XUE H X, et al. Nephropathy and hepatopathy in weaned piglets provoked by natural ochratoxin A and involved mechanisms[J]. Experimental and Toxicologic Pathology, 2016, 68(4):205-213.

DOI PMID

[41]
XUE J J, XIE L, LIU B, et al. Dietary supplementation of EGF ameliorates the negatively effects of LPS on early-weaning piglets:from views of growth performance,nutrient digestibility,microelement absorption and possible mechanisms[J]. Animals:an Open Access Journal from MDPI, 2021, 11(6):1598.

[42]
ZHANG H W, ZHANG B X, ZHANG X M, et al. Effects of cathelicidin-derived peptide from reptiles on lipopolysaccharide-induced intestinal inflammation in weaned piglets[J]. Veterinary Immunology and Immunopathology, 2017,192:41-53.

[43]
HUANG B, XIAO D F, TAN B, et al. Chitosan oligosaccharide reduces intestinal inflammation that involves calcium-sensing receptor (CaSR) activation in lipopolysaccharide (LPS)-challenged piglets[J]. Journal of Agricultural and Food Chemistry, 2016, 64(1):245-252.

DOI PMID

[44]
HOU Y Q, WANG L, DING B Y, et al. Dietary α-ketoglutarate supplementation ameliorates intestinal injury in lipopolysaccharide-challenged piglets[J]. Amino Acids, 2010, 39(2):555-564.

[45]
CHEN S K, LIU Y L, WANG X Y, et al. Asparagine improves intestinal integrity,inhibits TLR4 and NOD signaling,and differently regulates p38 and ERK1/2 signaling in weanling piglets after LPS challenge[J]. Innate Immunity, 2016, 22(8):577-587.

[46]
XIAO K, JIAO L, CAO S, et al. Whey protein concentrate enhances intestinal integrity and influences transforming growth factor- β1 and mitogen-activated protein kinase signalling pathways in piglets after lipopolysaccharide challenge[J]. British Journal of Nutrition, 2016, 115(6):984-993.

[47]
WANG H B, LIU Y L, SHI H F, et al. Aspartate attenuates intestinal injury and inhibits TLR4 and NODs/NF-κB and p38 signaling in weaned pigs after LPS challenge[J]. European journal of nutrition, 2017, 56(4):1433-1443.

DOI PMID

[48]
WAITITU S M, YIN F G, PATTERSON R, et al. Short-term effect of supplemental yeast extract without or with feed enzymes on growth performance,immune status and gut structure of weaned pigs challenged with Escherichia coli lipopolysaccharide[J]. Journal of animal science and biotechnology, 2016,7:64.

[49]
JIAO L F, WANG C C, WU H, et al. Copper/zinc-loaded montmorillonite influences intestinal integrity,the expression of genes associated with inflammation,TLR4-MyD88 and TGF-β1 signaling pathways in weaned pigs after LPS challenge[J]. Innate Immunity, 2017, 23(8):648-655.

[50]
ZHU C, WU Y P, JIANG Z Y, et al. Dietary soy isoflavone attenuated growth performance and intestinal barrier functions in weaned piglets challenged with lipopolysaccharide[J]. International Immunopharmacology, 2015, 28(1):288-294.

DOI PMID

[51]
FAN C, HAN J, LIU X, et al. Modulation of hypoxia-inducible factor-1α/cyclo-oxygenase-2 pathway associated with attenuation of intestinal mucosa inflammatory damage by Acanthopanax senticosus polysaccharides in lipopolysaccharide-challenged piglets[J]. British Journal of Nutrition, 2019, 122(6):666-675.

[52]
AHASAN A S M L, INVERNIZZI G, FARINA G, et al. The effects of superoxide dismutase-rich melon pulp concentrate on inflammation,antioxidant status and growth performance of challenged post-weaning piglets[J]. Animal, 2019, 13(1):136-143.

[53]
MAO X F, PIAO X S, LAI C H, et al. Effects of beta-glucan obtained from the Chinese herb Astragalus membranaceus and lipopolysaccharide challenge on performance,immunological,adrenal,and somatotropic responses of weanling pigs[J]. Journal of Animal Science, 2005, 83(12):2775-2782.

[54]
姚淑红. 猪大肠杆菌病及其流行特点[J]. 山东畜牧兽医, 2016, 37(6):32.

YAO S H. Escherichia coli disease in pigs and its epidemiological characteristics[J]. Shandong Journal of Animal Science and Veterinary Medicine, 2016, 37(6):32. (in Chinese)

[55]
贾良梁. 猪肠型大肠杆菌病的发病机制[J]. 国外畜牧学(猪与禽), 2018, 38(10):1-5.

JIA L L. Swine enteric colibacillosis:diagnosis,therapy and antimicrobial resistance[J]. Animals Science Abroad (Pigs and Poultry), 2018, 38(10):1-5. (in Chinese)

[56]
袁晴晴, 喻礼怀, 董丽. 霉菌毒素对猪肠道健康的影响及其营养调控[J]. 动物营养学报, 2024, 36(4):2118-2127.

DOI

YUAN Q Q, YU L H, DONG L. Effects of mycotoxins on intestinal health and its nutritional regulation in pigs[J]. Chinese Journal of Animal Nutrition, 2024, 36(4):2118-2127. (in Chinese)

DOI

[57]
KUIPER-GOODMAN T, SCOTT P M. Risk assessment of the mycotoxin ochratoxin A[J]. Biomedical and Environmental Sciences, 1989, 2(3):179-248.

[58]
KHOURY A E, ATOUI A. Ochratoxin A:general overview and actual molecular status[J]. Toxins, 2010, 2(4):461-493.

[59]
YING C, HONG W, NIANHUI Z, et al. Nontoxic concentrations of OTA aggravate DON-induced intestinal barrier dysfunction in IPEC-J2 cells via activation of NF-κB signaling pathway[J]. Toxicology Letters, 2019,311:114-124.

[60]
YANG S H, LI L, YU L H, et al. Selenium-enriched yeast reduces caecal pathological injuries and intervenes changes of the diversity of caecal microbiota caused by ochratoxin-A in broilers[J]. Food and Chemical Toxicology, 2020,137:111139.

[61]
MARIN D E, TARANU I. Ochratoxin A and its effects on immunity[J]. Toxin Reviews, 2015, 34(1):11-20.

[62]
ALVAREZ-ERVITI L, LEACHE C, GONZÁLEZ-PEÑAS E, et al. Alterations induced in vitro by ochratoxin A in rat lymphoid cells[J]. Human & Experimental Toxicology, 2005, 24(9):459-466.

[63]
张薇, 牛军龙, 郭永鹏, 等. 呕吐毒素对猪肠道屏障的影响及其营养调控研究进展[J]. 动物营养学报, 2022, 34(10):6249-6256.

DOI

ZHANG W, NIU J L, GUO Y P, et al. Research progress of effects of deoxynivalenol on intestinal barrier and its nutritional regulation in pigs[J]. Chinese Journal of Animal Nutrition, 2022, 34(10):6249-6256. (in Chinese)

DOI

[64]
BECKER C, REITER M, PFAFFL M W, et al. Expression of immune relevant genes in pigs under the influence of low doses of deoxynivalenol (DON)[J]. Mycotoxin Research, 2011, 27(4):287-293.

DOI PMID

[65]
HAO Y, XING M J, GU X H. Research progress on oxidative stress and its nutritional regulation strategies in pigs[J]. Animals, 2021, 11(5):1384.

[66]
CAO S T, WANG C C, YAN J T, et al. Curcumin ameliorates oxidative stress-induced intestinal barrier injury and mitochondrial damage by promoting Parkin dependent mitophagy through AMPK-TFEB signal pathway[J]. Free Radical Biology and Medicine, 2020,147:8-22.

[67]
YU L H, LI H M, PENG Z, et al. Early weaning affects liver antioxidant function in piglets[J]. Animals, 2021, 11(9):2679.

[68]
UPADHAYA S D, KIM I H. The impact of weaning stress on gut health and the mechanistic aspects of several feed additives contributing to improved gut health function in weanling piglets-a review[J]. Animals, 2021, 11(8):2418.

[69]
SU W F, GONG T, JIANG Z P, et al. The role of probiotics in alleviating postweaning diarrhea in piglets from the perspective of intestinal barriers[J]. Frontiers in Cellular and Infection Microbiology, 2022,12:883107.

[70]
陈祥兴, 张崇玉, 黄丽波, 等. 镰刀菌毒素对断奶仔猪肠道IL-1β和IL-6分布和表达的影响[J]. 畜牧兽医学报, 2016, 47(10):2126-2135.

CHEN X X, ZHANG C Y, HUANG L B, et al. Effects of fusarium toxins on IL-1β and IL-6 in post-weaning piglets[J]. Acta Veterinaria et Zootechnica Sinica, 2016, 47(10):2126-2135. (in Chinese)

[71]
MCCRACKEN B A, SPURLOCK M E, ROOS M A, et al. Weaning anorexia may contribute to local inflammation in the piglet small intestine[J]. The Journal of Nutrition, 1999, 129(3):613-619.

[72]
SPREEUWENBERG M A, VERDONK J M, GASKINS H R, et al. Small intestine epithelial barrier function is compromised in pigs with low feed intake at weaning[J]. The Journal of Nutrition, 2001, 131(5):1520-1527.

[73]
PIÉ S, LALLÈS J P, BLAZY F, et al. Weaning is associated with an upregulation of expression of inflammatory cytokines in the intestine of piglets[J]. The Journal of Nutrition, 2004, 134(3):641-647.

[74]
HU C H, XIAO K, LUAN Z S, et al. Early weaning increases intestinal permeability,alters expression of cytokine and tight junction proteins,and activates mitogen-activated protein kinases in pigs[J]. Journal of Animal Science, 2013, 91(3):1094-1101.

[75]
DENG Q Q, TAN X, WANG H R, et al. Changes in cecal morphology,cell proliferation,antioxidant enzyme,volatile fatty acids,lipopolysaccharide,and cytokines in piglets during the postweaning period[J]. Journal of Animal Science, 2020, 98(3):skaa046.

[76]
DE GROOT N, FARIÑAS F, CABRERA-GÓMEZ C G, et al. Weaning causes a prolonged but transient change in immune gene expression in the intestine of piglets[J]. Journal of Animal Science, 2021, 99(4):skab065.

[77]
YI H B, JIANG D H, ZHANG L, et al. Developmental expression of STATs,nuclear factor-κB and inflammatory genes in the jejunum of piglets during weaning[J]. International Immunopharmacology, 2016,36:199-204.

[78]
CAO S T, HOU L, SUN L H, et al. Intestinal morphology and immune profiles are altered in piglets by early-weaning[J]. International immunopharmacology, 2022,105:108520.

[79]
ZHONG X, ZHANG Z W, WANG S J, et al. Microbial-driven butyrate regulates jejunal homeostasis in piglets during the weaning stage[J]. Frontiers in Microbiology, 2018,9:3335.

[80]
AL-SADI R, BOIVIN M, MA T. Mechanism of cytokine modulation of epithelial tight junction barrier[J]. Frontiers in Bioscience (Landmark Edition), 2009,14:2765-2778.

[81]
LIU Y L, HUANG J J, HOU Y Q, et al. Dietary arginine supplementation alleviates intestinal mucosal disruption induced by Escherichia coli lipopolysaccharide in weaned pigs[J]. British Journal of Nutrition, 2008, 100(3):552-560.

文章导航

/