研究论文

低聚壳聚糖硒通过调控转化生长因子-β1/Smads信号通路减轻玉米赤霉烯酮对断奶仔猪肠道损伤的影响

  • 李坤 ,
  • 佘福泽 ,
  • 葛昆陇 ,
  • 张建斌 ,
  • 李留安 ,
  • 秦顺义 , *
展开
  • 天津农学院动物科学与动物医学学院,天津市农业动物繁育与健康养殖重点实验室,天津 300392
*秦顺义,副教授,硕士生导师,E-mail:

李坤(1998—),女,天津人,硕士研究生,研究方向为临床兽医学。E-mail:

Copy editor: 陈鑫

收稿日期: 2024-11-30

  网络出版日期: 2025-06-12

基金资助

天津市生猪现代农业产业技术体系创新团队-功能饲料岗位(ITTPRS2025006)

天津市科技计划项目(23ZYCGSN00190)

Chitosan Oligosaccharide Selenium Attenuates Effects of Zearalenone on Intestinal Damage in Weaned Piglets by Modulating Transforming Growth Factor-β1/Smads Signaling Pathway

  • LI Kun ,
  • SHE Fuze ,
  • GE Kunlong ,
  • ZHANG Jianbin ,
  • LI Liuan ,
  • QIN Shunyi , *
Expand
  • Tianjin Key Laboratory of Agricultural Animal Breeding and Health Breeding, College of Animal Science and Veterinary Medicine, Tianjin Agricultural University, Tianjin 300392, China
* associate professor, E-mail:

Received date: 2024-11-30

  Online published: 2025-06-12

摘要

本试验旨在探究低聚壳聚糖硒通过调控转化生长因子-β1/Smads(TGF-β1/Smads)信号通路缓解玉米赤霉烯酮(ZEA)对断奶仔猪肠道损伤的影响。选取健康的35日龄断奶仔猪60头,随机分为4组,每组5个重复,每个重复3头仔猪。C组饲喂基础饲粮,Z组饲喂基础饲粮+2 mg/kg ZEA,ZS1组饲喂基础饲粮+2 mg/kg ZEA+0.3 mg/kg低聚壳聚糖硒,ZS2组饲喂基础饲粮+2 mg/kg ZEA+0.5 mg/kg低聚壳聚糖硒。预试期7 d,正试期42 d。试验结束后,测定空肠屏障功能相关基因的mRNA表达水平、抗氧化指标、免疫指标以及测定TGF-β1/Smad信号通路相关基因的mRNA表达水平和相关蛋白的表达。结果表明:1)与C组相比,添加ZEA显著或极显著降低仔猪空肠组织的闭锁小带蛋白-1(ZO-1)、闭合蛋白(Occludin)、封密蛋白-3(Claudin-3)的mRNA相对表达量,白细胞介素-10(IL-10)含量,谷胱甘肽过氧化物酶(GSH-Px)活性、总抗氧化能力(T-AOC)及总超氧化物歧化酶(T-SOD)活性(P<0.05或P<0.01),极显著升高肿瘤坏死因子-α(TNF-α)、白细胞介素-1β(IL-1β)和白细胞介素-6(IL-6)及丙二醛(MDA)含量(P<0.01);与Z组相比,添加低聚壳聚糖硒可显著或极显著增加空肠组织ZO-1、OccludinClaudin-3的mRNA相对表达量,IL-10含量,T-AOC以及T-SOD和GSH-Px活性(P<0.05或P<0.01),极显著降低IL-6、IL-1β及MDA含量(P<0.01)。2)与C组相比,添加ZEA显著或极显著升高仔猪空肠组织的转化生长因子-β1(TGF-β1)与Smad3的mRNA相对表达量以及P-Smad2/3/Smad2/3和TGF-β1蛋白表达量(P<0.05或P<0.01),极显著降低Smad7的mRNA相对表达量以及蛋白表达量(P<0.01);与Z组相比,添加低聚壳聚糖硒可显著或极显著降低空肠组织的TGF-β1、Smad2以及Smad3的mRNA相对表达量(P<0.05或P<0.01),显著或极显著增加Smad7的mRNA相对表达量以及蛋白表达量(P<0.05或P<0.01),显著降低P-Smad2/3/Smad2/3和TGF-β1蛋白表达量(P<0.05)。由此可知,低聚壳聚糖硒能够通过调控TGF-β1/Smads信号通路,改善空肠屏障损伤、减轻空肠组织炎症反应、调节空肠抗氧化功能,进而缓解饲喂ZEA对仔猪空肠的损伤。

本文引用格式

李坤 , 佘福泽 , 葛昆陇 , 张建斌 , 李留安 , 秦顺义 . 低聚壳聚糖硒通过调控转化生长因子-β1/Smads信号通路减轻玉米赤霉烯酮对断奶仔猪肠道损伤的影响[J]. 动物营养学报, 2025 , 37(6) : 3633 -3643 . DOI: 10.12418/CJAN2025.299

Abstract

To investigate the effects of chitosan oligosaccharide selenium on intestinal damage in weaned piglets by alleviating zearalenone (ZEA) containing intestinal damage through modulation of the transforming growth factor-β1 (TGF-β1)/Smads signaling pathway. Sixty healthy 35-day-old weaned piglets were selected and randomly divided into four groups, group C fed a basal diet, group Z fed the basal diet+2 mg/kg ZEA, group ZS1 fed the basal diet+2 mg/kg ZEA+0.3 mg/kg selenized-oligochitosan, and group ZS2 fed the basal diet+2 mg/kg ZEA+0.5 mg/kg selenized-oligochitosan. The pre-test period was 7 days and the formal test period was 42 days. At the end of the test, mRNA expression levels of genes related to jejunal barrier function, antioxidant indexes, and immune indexes were determined, as well as mRNA expression levels of genes related to the TGF-β1/Smads signaling pathway and expression of related proteins were measured. The results showed as follows: 1) compared with group C, ZEA could significantly or extremely significantly decrease the mRNA relative expression levels of zonula occludens-1(ZO-1), Occludin, and Claudin-3 in the jejunal of piglets, as well as interleukin-10 (IL-10) content and glutathione peroxidase (GSH-Px) activity, total antioxidant capacity(T-AOC), and total superoxide dismutase (T-SOD) activity (P<0.05 or P<0.01); meanwhile, it could extremely significantly increase the contents of tumor necrosis factor-α (TNF-α), interleukin-1β (IL-1β), and interleukin-6 (IL-6), as well as the content of malondialdehyde (MDA) (P<0.01). However, compared with group Z, the addition of chitosan oligosaccharide selenium could significantly or extremely significantly increase the mRNA relative expression levels of ZO-1, Occludin, and Claudin-3, the content of IL-10, T-AOC, and the activities of T-SOD and GSH-Px (P<0.05 or P<0.01); it could also extremely significantly decrease the contents of IL-6 and IL-1β, as well as the content of MDA (P<0.01). 2) Compared with group C, ZEA could significantly or extremely significantly increase the mRNA relative expression levels of transforming growth factor-β (TGF-β1) and Smad3, as well as the protein expression levels of P-Smad2/3/Smad2/3 and TGF-β1 in the jejunum of piglets (P<0.05 or P<0.01); it also could extremely significantly decrease the mRNA relative expression level and protein expression level of Smad7 (P<0.01). However, the addition of chitosan oligosaccharide selenium could significantly or extremely significantly decrease the mRNA relative expression levels of TGF-β1, Smad2, and Smad3 (P<0.05 or P<0.01). It could also significantly or extremely significantly increase the mRNA relative expression level and protein expression level of Smad7 (P<0.05 or P<0.01). Furthermore, it could significantly decrease the protein expression levels of P-Smad2/3/Smad2/3 and TGF-β1(P<0.05). In conclusion,chitosan oligosaccharide selenium can ameliorate jejunal barrier injury, attenuate jejunal tissue inflammation, and regulate jejunal antioxidant function by modulating the TGF-β1/Smads signaling pathway, thereby mitigating the damage to the jejunum of piglets induced by ZEA feeding.

玉米赤霉烯酮(zearalenone,ZEA)是一种类雌激素化合物,是谷类作物中镰刀菌的次生代谢产物,主要由禾谷镰刀菌等真菌产生[1],主要存在于霉变的玉米、小麦、高粱等谷物中,在畜禽饲料中是一种普遍存在的有毒物质,也是威胁力最大的污染霉菌毒素之一,对动物及人类健康造成严重的安全隐患,并给畜牧业造成巨大的经济损失。研究表明,ZEA能够诱导氧化应激与细胞凋亡[2],肝脏功能受损以及肠道稳态和屏障功能受到影响[3-4]。硒作为机体必需的微量元素,具有抗氧化及改善肠道菌群失调和肠道炎症的作用[5]。壳聚糖有抗炎、抗氧化和提高生产性能的作用,壳聚糖硒是将硒用化学的方法结合到壳聚糖分子上,而低聚壳聚糖硒是相对分子质量较小的壳聚糖硒,具有有机硒和低聚壳聚糖双重功能,有助于增强机体的抗氧化能力、调节免疫反应、提高机体抵抗力、改善动物的肠道健康和提高动物生产性能等[6]。相较于传统的壳聚糖硒,低聚壳聚糖硒展现出更优越的溶解能力和生物活性,这使得低聚壳聚糖硒在实际应用中的效果超越了普通的壳聚糖硒。韩婧娥等[7]研究表明,低聚壳聚糖硒能够改善蛋鸡生产性能,增强蛋鸡血浆及鸡蛋的抗氧化功能,调节盲肠肠道菌群。有研究表明,ZEA对性成熟前公猪性腺具有毒性作用[8],且对母猪的繁殖功能造成损害[9]。陈祥兴等[10]研究表明,ZEA能够影响仔猪肠道白细胞介素-1β(IL-1β)和白细胞介素-6(IL-6)的表达。傅春妮等[11]研究发现,低聚壳聚糖硒能减轻ZEA对猪小肠上皮细胞造成的损伤。
转化生长因子-β(TGF-β)被定义为一种具有多种功能的细胞因子,能够调控肠黏膜细胞的生长、分化、迁移以及上皮细胞的复原等[12],Smad蛋白在TGF-β1作用的同时发挥重要作用,可参与调节信号转导,激活后可抑制上皮细胞生长[13]。研究表明,TGF-β1在恢复肠道屏障的完整性方面起到了关键作用[14],且已有研究表明,ZEA能够对肠道屏障的完整性造成损害[15],进而损害机体健康并影响动物生产性能[16]。前期研究已证实,添加低聚壳聚糖硒能够有效缓解ZEA引起的断奶仔猪生长性能的降低[6]。但目前低聚壳聚糖硒通过调控TGF-β1/Smads信号通路减轻ZEA对仔猪肠道损伤的研究鲜见报导。因此,本试验通过检测肠道TGF-β1/Smads信号通路变化、抗氧化功能、屏障功能以及肠道炎症反应初步探索低聚壳聚糖硒通过调控肠道TGF-β1/Smads信号通路减轻ZEA对仔猪肠道损伤作用的可能机制,为低聚壳聚糖硒的应用提供参考。

1 材料与方法

1.1 试验材料

低聚壳聚糖硒为天津农学院动物医学实验教学中心实验室配制,硒含量为22.18 g/kg;ZEA纯度为98%。

1.2 试验设计与饲养管理

选取35日龄健康的“杜×长×大”三元杂交断奶仔猪60头为研究对象,将其随机划分为4组,每组5个重复,每个重复3头仔猪。C组仔猪饲喂基础饲粮,Z组仔猪饲喂基础饲粮+2 mg/kg ZEA,ZS1组仔猪饲喂基础饲粮+2 mg/kg ZEA+0.3 mg/kg低聚壳聚糖硒,ZS2组仔猪饲喂基础饲粮+2 mg/kg ZEA+0.5 mg/kg低聚壳聚糖硒。依据《猪饲养标准》(NY/T 65—2004)配制基础饲粮,其组成及营养水平见表1
表1 基础饲粮组成及营养水平(风干基础)

Table 1 Composition and nutrient levels of basal diets (air-dry basis) %

项目
Items
体重Body weight
8 to 20 kg 20 to 35 kg
原料Ingredients
玉米Corn 69.35 69.38
豆粕Soybean meal 13.00 14.00
大豆油Soybean oil 1.00 1.00
玉米蛋白粉Corn protein meal 5.00 7.00
小麦麸Wheat bran 4.00 4.00
鱼粉Fish meal 3.00
磷酸氢钙CaHPO4 1.00 1.20
石粉Limestone 1.00 0.80
预混料Premix1) 2.00 2.00
食盐NaCl 0.15 0.12
赖氨酸Lys 0.50 0.50
合计Total 100.00 100.00
营养水平Nutrient levels2)
消化能DE/(MJ/kg) 13.17 13.17
粗蛋白质CP 18.17 17.35
钙Ca 0.77 0.63
总磷TP 0.58 0.54
赖氨酸Lys 1.24 1.13
蛋氨酸Met 0.33 0.31

1)预混料为每千克饲粮提供 Premix provided the following per kg of diets:VA 12 000 IU,VD3 4 000 IU,VE 40 IU,VK3 3.0 mg,VB1 4.0 mg,VB2 10.0 mg,VB6 10 mg,VB12 0.04 mg,Fe(as ferrous sulfate)100 mg,Mn (as manganese sulfate)20 mg,Zn (as zinc sulfate) 100 mg,Cu (as copper sulfate) 8.0 mg,I (as Iodine sulfate) 0.2 mg,Se (as sodium selenite) 0.1 mg,叶酸 folic acid 1.0 mg,烟酸 niacin acid 40 mg,泛酸 pantothenic acid 20 mg,生物素 biotin 0.2 mg,胆碱 choline 800 mg。
2)参照GB/T 6432—2018方法测定CP含量,参照GB/T 6437—2018方法测定TP含量,参照GB/T 13885—2017方法测定Ca含量,参照GB/T 18246—2019方法测定氨基酸含量;DE参照GB/T 39235—2020计算得出。CP content was determined according to the method specified in GB/T 6432—2018, the TP content was determined according to the method specified in GB/T 6437—2018, the Ca content was determined according to the method specified in GB/T 13885—2017, and the amino acid content was determined according to the method specified in GB/T 18246—2019; DE was calculated according to the method specified in GB/T 39235—2020.

饲养过程中仔猪自由采食和饮水,并进行常规免疫程序和饲养管理。预试期7 d,正试期42 d。本研究涉及活体动物的试验设计及试验方法均通过天津农学院实验动物伦理委员会审核批准(批准号:2021LLSC29)。

1.3 样品采集

饲养试验结束后,将所有仔猪全部处死,分离空肠,一部分保存于4%多聚甲醛中,用于研究组织形态学,一部分保存于液氮中,用于检测分子生物学指标。

1.4 测定指标及方法

1.4.1 肠道屏障功能指标测定

采用实时荧光定量PCR(qRT-PCR)法,取冻存空肠组织,加入裂解液研磨匀浆,12 000×g、4 ℃离心10 min,取上清,按照上海碧云天生物技术有限公司的RNAeasy动物RNA抽提试剂盒(离心柱式)说明书说明提取肠道组织总RNA,RNA的浓度用A260/A280进行定量,按照反转录试剂盒要求合成cDNA。使用美国BIO-RED公司的CFX Connect荧光定量PCR仪检测肠道组织闭合蛋白(Occludin)、封闭蛋白-3(Claudin-3)和闭锁小带蛋白-1(ZO-1)的mRNA相对表达量,内参基因为β-肌动蛋白。扩增条件为:预变性95 ℃ 3 min,1个循环;扩增95 ℃ 5 s,60 ℃ 20 s,40个循环。引物序列见表2。采用2-△△Ct法计算目的基因mRNA相对表达量。
表2 引物序列

Table 2 Primer sequence

基因
Genes
引物序列
Primer sequence (5'—3')
产物长度
Product length/bp
闭合蛋白Occludin F:AGTGGTAACTTGGAGGCGTCTTC
R:TCTGTCTCGTAATGGTCTTGCTCTG
92
封闭蛋白-3 Claudin-3 F:TGCTGCTTCTCTCTGCCTTCTG
R:GCCTTGGTGTTGGGTAAGATGTTG
83
闭锁小带蛋白-1 ZO-1 F:GGCGAAGGTAATTCAGTGTCATTGG
R:AGTATCTTCTCGGTTTGGTGGTCTG
114
转化生长因子-β1 TGF-β1 F:TGGCTGACCCGCAGAGAGG
R:CGTGGAGTGTGTTATCTTTGCTGTC
82
Smad2 F:GTCGTCCATCCTGCCCTTCAC
R:GCCTTCTCGCACCACTTCTCC
99
Smad3 F:ACGACTACAGCCATTCCATCC
R:TTCTCCATCTTCACTCAGGTAGC
110
Smad7 F:GAGGCTGTGTTGCTGTGAATCTTAC
R:GCAGAGTCGGCTAAGGTGATGG
82
β-肌动蛋白β-actin F:TCGAGACCTTCAACACCCCAG
R:GTCTCCGGAGTCCATCACGA
101

1.4.2 肠道抗氧化指标测定

采用南京建成生物工程研究所的试剂盒对仔猪空肠组织总抗氧化能力(T-AOC),谷胱甘肽过氧化物酶(GSH-Px)、总超氧化物歧化酶(T-SOD)活性和丙二醛(MDA)含量进行测定。

1.4.3 肠道免疫指标测定

取冻存空肠组织,加入预冷磷酸盐缓冲液(PBS)研磨匀浆,3 000×g、4 ℃离心15 min,取上清液。采用江苏酶免实业有限公司的酶联免疫吸附测定(ELISA)试剂盒检测肠道组织匀浆上清液中IL-1β、IL-6、白细胞介素-10(IL-10)和肿瘤坏死因子-α(TNF-α)含量。

1.4.4 肠道组织TGF-β1/Smads信号通路mRNA表达的测定

采用qRT-PCR法,取冻存肠道组织,加入裂解液研磨匀浆,12 000×g、4 ℃离心10 min,取上清液,按照上海碧云天生物技术有限公司的RNAeasy动物RNA抽提试剂盒(离心柱式)的说明书提取肠道组织总RNA,RNA的浓度用A260/A280进行定量,按照反转录试剂盒要求合成cDNA。使用美国BIO-RED公司的CFX Connect荧光定量PCR仪检测肠道组织TGF-β1、Smad2、Smad3以及Smad7的mRNA相对表达量,扩增条件为:预变性95 ℃ 3 min,1个循环;扩增95 ℃ 5 s,60 ℃ 20 s,40个循环。引物序列见表2。采用2-△△Ct法计算目的基因mRNA相对表达量。

1.4.5 肠道组织TGF-β1/Smads信号通路蛋白表达的测定

采用Western blotting法,取冻存空肠组织,加入RIPA裂解液,充分均浆,4 ℃、12 000×g离心10 min,取上清液,采用BCA法测定蛋白浓度。120 V恒定电压进行电泳,用转膜仪15 V转膜45 min,用封闭液(5%脱脂奶粉)4 ℃封闭2 h,分别稀释TGF-β1(1∶2 000)、Smad2/3(1∶1 000)、P-smad2/3(1∶1 000)、Smad7(1∶2 000)以及β-肌动蛋白(1∶5 000)的一抗4 ℃孵育过夜,室温下用含Tween 20的Tris缓冲盐溶液(TBST)洗膜,羊抗兔抗体(1∶5 000)室温孵育2 h,洗膜后用北京索莱宝科技有限公司ECL超敏发光液发光显影,Image Lab 5.0软件定量分析条带灰度值,结果采用Graph Prism10.0软件绘图。

1.5 数据统计分析

试验数据采用SPSS 27.0统计软件进行单因素方差分析,并采用Duncan氏法进行组间平均值多重比较,P<0.05表示差异显著,P<0.01表示差异极显著。采用GraphPad Prism 10.0软件绘图。

2 结果与分析

2.1 低聚壳聚糖硒缓解ZEA对仔猪肠道屏障功能的影响

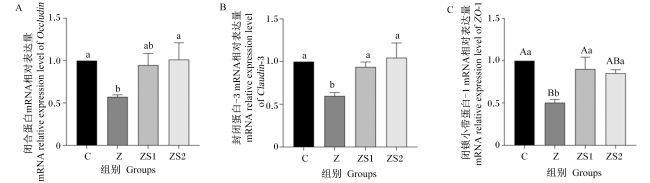
图1可知,与C组相比,Z组仔猪空肠的OccludinCluadin-3以及ZO-1的mRNA相对表达量均显著或极显著降低(P<0.05或P<0.01);与Z组相比,ZS1组或ZS2组OccludinCluadin-3以及ZO-1的mRNA相对表达量均显著或极显著升高(P<0.05或P<0.01)。
图1 低聚壳聚糖硒缓解ZEA对仔猪空肠OccludinClaudin-3以及ZO-1的mRNA相对表达量的影响

不同大写字母表示差异极显著(P<0.01),不同小写字母表示差异显著(P<0.05),相同字母或无字母表示差异不显著(P>0.05)。下图同。

Fig.1 Effects of selenium oligosaccharide alleviation of ZEA on mRNA relative expression levels of Occludin, Claudin-3, and ZO-1 in jejunum of piglets

Different uppercase letters indicate very significant difference (P<0.01), different lowercase letters indicate significant difference (P<0.05), and the same or no letters indicate no significant difference (P>0.05). The same as below.

2.2 低聚壳聚糖硒缓解ZEA对仔猪肠道抗氧化功能的影响

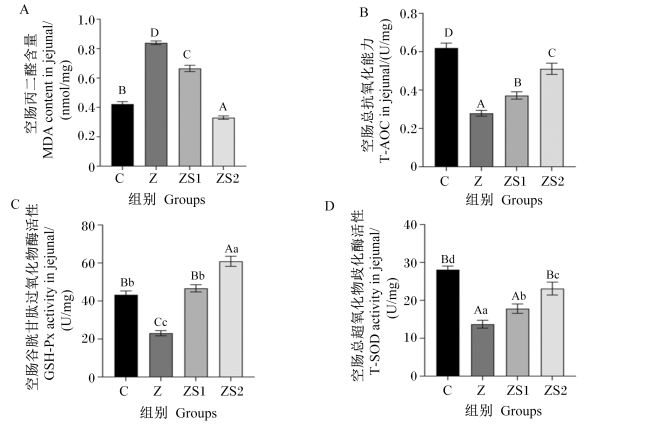
图2可知,与C组相比,Z组仔猪空肠的T-AOC,T-SOD、GSH-Px活性极显著降低(P<0.01),MDA含量极显著升高(P<0.01);与Z组相比,ZS1组与ZS2组仔猪空肠的T-AOC,T-SOD、GSH-Px活性均显著或极显著升高(P<0.05或P<0.01),MDA含量极显著降低(P<0.01)。
图2 低聚壳聚糖硒缓解ZEA对仔猪空肠T-AOC,GSH-Px、T-SOD活性以及MDA含量的影响

Fig.2 Effects of selenium oligosaccharide alleviation of ZEA on T-AOC, GSH-Px, T-SOD activities and MDA content in jejunum of piglets

2.3 低聚壳聚糖硒缓解ZEA对仔猪肠道免疫功能的影响

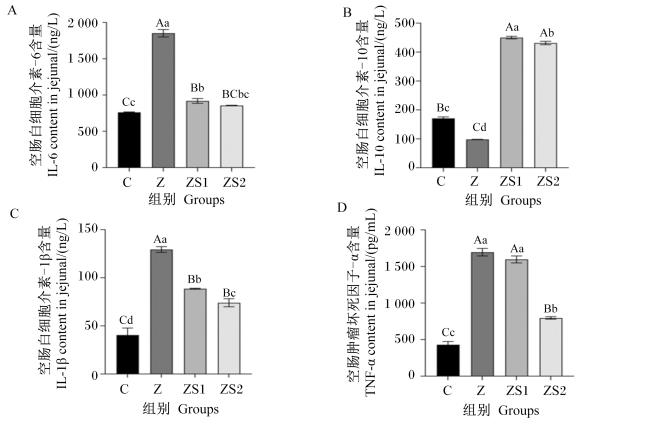
图3可知,与C组相比,Z组仔猪空肠的IL-6、IL-1β以及TNF-α含量均极显著升高(P<0.01),IL-10含量极显著降低(P<0.01);与Z组相比,ZS1组与ZS2组的IL-6与IL-1β含量极显著降低(P<0.01),IL-10含量极显著升高(P<0.01);ZS2组较ZS1组的TNF-α含量极显著降低(P<0.01)。
图3 低聚壳聚糖硒缓解ZEA对仔猪空肠IL-6、IL-10、IL-1β以及TNF-α含量的影响

Fig.3 Effects of selenium oligosaccharide alleviation of ZEA on IL-6, IL-10, IL-1β and TNF-αcontents in jejunum of piglets

2.4 低聚壳聚糖硒缓解ZEA对仔猪空肠TGF-β1、Smad2、Smad3以及Smad7的mRNA相对表达量的影响
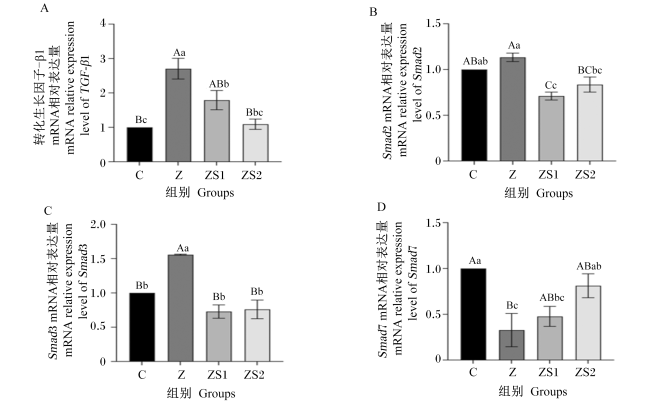
图4可知,与C组相比,Z组仔猪空肠的TGF-β1与Smad3的mRNA相对表达量极显著升高(P<0.01),Smad7的mRNA相对表达量极显著降低(P<0.01);与Z组相比,ZS1组与ZS2组的TGF-β1、Smad2以及Smad3的mRNA相对表达量均显著或极显著降低(P<0.05或P<0.01),Smad7的mRNA相对表达量显著或极显著升高(P<0.05或P<0.01)。
图4 低聚壳聚糖硒缓解ZEA对仔猪空肠TGF-β1、Smad2、Smad3以及Smad7的mRNA相对表达量的影响

Fig.4 Effects of selenium oligosaccharide alleviation of ZEA on mRNA relative expression levels of TGF-β1, Smad2, Smad3, and Smad7 in jejunum of piglets

2.5 低聚壳聚糖硒缓解ZEA对仔猪空肠TGF-β1、Smad2/3、P-Smad2/3以及Smad7蛋白相对表达量的影响
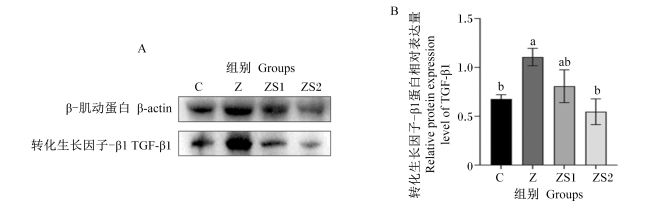
图5可知,与C组相比,Z组仔猪空肠的TGF-β1蛋白相对表达量显著升高(P<0.05);与Z组相比,ZS1组TGF-β1蛋白相对表达量差异不显著(P>0.05),ZS2组TGF-β1蛋白相对表达量显著降低(P<0.05)。
图5 低聚壳聚糖硒缓解ZEA对仔猪空肠TGF-β1蛋白相对表达量的影响

A:TGF-β1的蛋白条带图;B:TGF-β1的蛋白相对表达量。

Fig.5 Effects of selenium oligosaccharide alleviation of ZEA on TGF-β1 protein relative expression level in jejunum of piglets

A: protein band diagram of TGF-β1;B:protein relative expression level of TGF-β1.

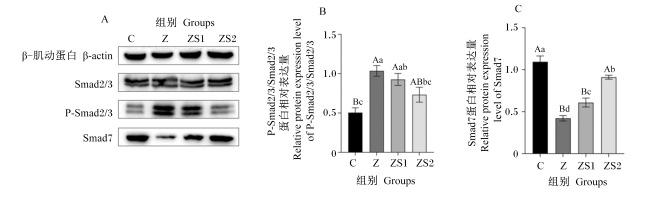
图6可知,与C组相比,Z组仔猪空肠的P-Smad2/3/Smad2/3蛋白相对表达量极显著升高(P<0.01),Smad7的蛋白相对表达量极显著降低(P<0.01);与Z组相比,ZS2组的P-Smad2/3/Smad2/3蛋白相对表达量显著降低(P<0.05),ZS1组与ZS2组的Smad7蛋白相对表达量均显著或极显著升高(P<0.05或P<0.01)。
图6 低聚壳聚糖硒缓解ZEA对仔猪空肠Smad2/3、P-smad2/3以及Smad7蛋白相对表达量的影响

A:Smad2/3、P-Smad2/3以及Smad7的蛋白条带图;B、C:P-Smad2/3/Smad2/3以及Smad7的蛋白相对表达量。

Fig.6 Effects of selenium oligosaccharide alleviation of ZEA on Smad2/3,P-smad2/3 and Smad7 protein relative expression levels in jejunum of piglets

A:protein band diagram of Smad2/3, P-Smad2/3 and Smad7;B,C:protein relative expression levels of P-Smad2/3/Smad2/3 and Smad7.

3 讨论

TGF-β1在肠上皮细胞的增殖、分化以及肠黏膜损伤的修复过程中起到核心作用[17]。TGF-β与Ⅱ型受体2(TβR2)特异性结合,随后引发Ⅰ型受体(TβR1)的磷酸化并激活,两者结合形成复合体;接着,被激活的TβR1进一步磷酸化并激活Smad2和Smad3;之后,活化的Smad2、Smad3与Smad4相互结合,形成稳定的聚合体;最终,这一聚合体通过核转位机制进入细胞核内,直接参与并调控相关靶基因的表达。Smad7作为TGF-β/Smad信号传导路径的关键抑制因子,一方面,它能够与Smad2/3竞争性地争夺TGF-β1受体的结合位点,有效封锁受体与其他配体的结合途径,从而遏制Smad2/3的磷酸化激活过程;另一方面,Smad7还能直接干预Smad2/3/4的结合,阻止它们形成具有功能性的聚合体,进而在多个层面上阻断并削弱TGF-β1信号的生物学效应[18-19]。本研究指出,相较于C组,Z组中TGF-β1以及P-Smad2/3/Smad2/3的蛋白表达水平呈现显著增高,这一差异可能与生物体内部的自我调节机制紧密相关。有研究显示,当组织遭受损伤时,血小板会迅速积聚于损伤区域,并且这些血小板内含有高浓度的TGF-β1,随后,血小板通过脱颗粒等机制将大量的TGF-β1释放出来,这一过程对于加速伤口的愈合具有积极的促进作用[20]。当TGF-β1与TβR2相结合时,磷酸化作用会激活TβR1,并与其产生复合物,活化状态的TβR1经磷酸化后激活Smad2/3,进一步导致P-Smad2/3的表达水平上升,抑制TGF-β1/Smads通路,从而进一步加剧TGF-β1/Smads通路介导的肠黏膜上皮损伤的修复工作,肠道屏障损伤加剧。肠道屏障是人体同外源性物质接触的首道防线,而Claudin、Occludin和ZO-1是评估肠黏膜屏障的关键指标[21]。有研究表明,经过ZEA(20 μg/mL)培养24 h的仔猪空肠上皮细胞里的ZO-1、OccludinClaudin-3的mRNA相对表达量呈明显下降[22];王玉等[23]研究结果表明,当给仔猪饲喂添加低聚壳聚糖的饲粮后,仔猪空肠ZO-1和Occludin基因的表达水平得到显著提升;Liu等[24]研究表明,0.2、0.4、0.6 mg/kg硒代蛋氨酸可上调T-2毒素造成的ZO-1和Occludin的表达下降,减少兔空肠炎症。本研究发现,添加低聚壳聚糖硒能缓解由ZEA导致的仔猪空肠组织内这些蛋白表达水平的变化,表明低聚壳聚糖硒能够通过调控TGF-β1/Smads信号通路改善肠道屏障功能障碍。
此外,与C组相比,观察到Z组中Smad7的蛋白表达水平有所降低。Smad7作为TGF-β1/Smads信号传导通路的一个重要负调节因子,它通过与Smad2和Smad3竞争性地结合TGF-β1受体,来阻碍它们的磷酸化过程,从而实现对TGF-β1/Smads信号通路的抑制作用。此外,Smad7还被看作是TGF-β1激活后需要诱导表达的一个关键目标基因。在这个信号通路中,Smad7扮演着防止信号过度活化的重要角色,确保信号传导不会失控[25-26]。因此,Z组中Smad7表达的下降可能意味着TGF-β1/Smads信号通路的抑制作用减弱,这可能与该组中出现的TGF-β1和P-Smad2/3/Smad2/3蛋白表达量上升的现象相关联。本研究中,Z组TGF-β1、P-Smad2/3的蛋白表达升高,从而抑制了Smad7的表达,导致Smad7的蛋白表达量降低。
氧化损伤在多种器官纤维化的分子机制中具有重要作用[27],TGF-β1在纤维化过程中过度激活,促使胶原蛋白和ECM生成,TGF-β1/Smad信号通路的异常传导是导致多种组织纤维化的经典通路[28]。Wu等[29]研究结果表明,将ZEA添加到初情期前的母猪饲粮中,结果发现母猪的T-AOC及T-SOD活性明显降低;王欢欢等[30]研究结果表明,壳聚糖硒能够拮抗ZEA对仔猪肝脏和肾脏产生的氧化损伤;Gu等[31]研究表明,饲粮添加15 mg/kg壳聚糖可缓解脂多糖(LPS)诱导的蛋鸡肠道屏障损伤和氧化免疫应激。本研究结果表明,与C组相比,添加ZEA能够使空肠组织中MDA含量显著增加,T-AOC及GSH-Px、T-SOD活性下降;在加入低聚壳聚糖硒后,空肠T-SOD、GSH-Px活性以及T-AOC均有所提升,MDA含量下降,表明添加低聚壳聚糖硒能够通过调控TGF-β1/Smads信号通路缓解ZEA引起的仔猪肠道氧化损伤,增强仔猪抗氧化功能,减少空肠组织纤维化。
TGF-β信号通路在免疫调节过程中起着多种作用,作为免疫抑制及耐受性诱导因子在免疫细胞功能、发育、活化等方面起着多种调节作用[32-33]。研究表明,TGF-β信号通路失衡可能导致免疫系统对自身组织的攻击,导致炎症反应发生和组织损伤[32,34-35];有研究发现,TGF-β1的缺乏会引发新生小鼠产生多器官炎症反应,这些症状与自身免疫性疾病具有相似性[36]。本研究结果表明,与C组相比,Z组空肠IL-6、IL-1β以及TNF-α含量升高,IL-10含量下降;当加入低聚壳聚糖硒后,这种情况得到了显著的缓解,表明添加低聚壳聚糖硒可以有效地通过TGF-β1/Smad信号通路减轻由ZEA导致的仔猪肠道炎症,从而增强仔猪免疫功能。
综上所述,低聚壳聚糖硒通过调控TGF-β1/Smads信号通路,抑制相关基因和蛋白的表达,从而减轻由ZEA引起的肠道炎症反应,促进空肠抗氧化功能以及屏障功能的恢复,缓解空肠组织损伤。

4 结论

低聚壳聚糖硒能够通过调控TGF-β1/Smads信号通路减轻ZEA引起的断奶仔猪肠道损伤。
[1]
DROUAULT M, ROUGE M, HANOUX V, et al. Ex vivo effects of bisphenol A or zearalenone on the prepubertal rat testis[J]. Environmental Toxicology and Pharmacology, 2023,95:104203.

[2]
RAJENDRAN P, AMMAR R B, AL-SAEEDI F J, et al. Kaempferol inhibits zearalenone-induced oxidative stress and apoptosis via the PI3K/Akt-mediated Nrf2 signaling pathway:in vitro and in vivo studies[J]. International Journal of Molecular Sciences, 2020, 22(1):217.

[3]
WANG N, LI P, WANG M Y, et al. The protective role of Bacillus velezensis a2 on the biochemical and hepatic toxicity of zearalenone in mice[J]. Toxins, 2018, 10(11):449.

[4]
AKBARI P, BRABER S, VARASTEH S, et al. The intestinal barrier as an emerging target in the toxicological assessment of mycotoxins[J]. Archives of Toxicology, 2017, 91(3):1007-1029.

DOI PMID

[5]
陈冬梅, 吴博, 杨文庆. 硒营养状态对大鼠肠道菌群结构及炎症的影响[J]. 中国微生态学杂志, 2019, 31(3):291-296.

CHEN D M, WU B, YANG W Q. Effect of selenium nutrition on intestinal flora structure and inflammation in rats[J]. Chinese Journal of Microecology, 2019, 31(3):291-296.(in Chinese)

[6]
李鹏程, 彭玉凯, 余锐洁, 等. 低聚壳聚糖硒缓解玉米赤霉烯酮对仔猪生长性能、血浆生化、抗氧化及肠道菌群的影响[J]. 饲料研究, 2022, 45(15):31-35.

LI P C, PENG Y K, YU R J, et al. Oligochitosan-selenium alleviates effect of zearalenone on growth performance,plasma biochemical indexes,antioxidant function and intestinal flora of piglets[J]. Feed Research, 2022, 45(15):31-35.(in Chinese)

[7]
韩婧娥, 杨贵军, 张晓倩, 等. 低聚壳聚糖硒对蛋鸡生产性能、抗氧化功能及肠道菌群的影响[J]. 饲料研究, 2021, 44(17):23-26.

HAN J E, YANG G J, ZHANG X Q, et al. Effect of oligochitosan selenium on production performance,antioxidant function and intestinal flora of laying hens[J]. Feed Research, 2021, 44(17):23-26.(in Chinese)

[8]
刘泮竹, 尚重兴, 苟克勉, 等. 玉米赤霉烯酮对性成熟前公猪性腺的毒性作用及牛磺酸的保护功能[J]. 中国兽医科学, 2024, 54(12):1683-1691.

LIU P Z, SHANG C X, GOU K M, et al. Toxic effects of zearalenone on gonads of premature boars and protective functions of taurine[J]. Chinese Veterinary Science, 2024, 54(12):1683-1691.(in Chinese)

[9]
李守杰, 洪伟, 薛文娟. 玉米赤霉烯酮污染日粮添加膨润土对断奶仔猪生长性能、养分利用率及生殖器官发育的影响[J]. 中国饲料, 2019(2):39-44.

LI S J, HONG W, XUE W J. Effects of supplementation of bentone in zearalenone contaminative diets on growth performance,nutrient digestibility and development of reproduction organs of weaning pigs[J]. China Feed, 2019(2):39-44.(in Chinese)

[10]
陈祥兴, 张崇玉, 黄丽波, 等. 镰刀菌毒素对断奶仔猪肠道IL-1β和IL-6分布和表达的影响[J]. 畜牧兽医学报, 2016, 47(10):2126-2135.

CHEN X X, ZHANG C Y, HUANG L B, et al. Effects of Fusarium toxins on IL-1β and IL-6 in post-weaning piglets[J]. Acta Veterinaria et Zootechnica Sinica, 2016, 47(10):2126-2135.(in Chinese)

[11]
傅春妮, 李元辉, 李鹏程, 等. 低聚壳聚糖硒抵抗玉米赤霉烯酮诱导猪肠上皮细胞氧化损伤和内质网应激的作用研究[J]. 动物营养学报, 2021, 33(9):5226-5235.

DOI

FU C N, LI Y H, LI P C, et al. Effects of oligomeric chitosan selenium on oxidative damage and endoplasmic reticulum stress in zearalenon-induced pig intestinal epithelial cells[J]. Chinese Journal of Animal Nutrition, 2021, 33(9):5226-5235.(in Chinese)

[12]
ZHANG P F, JING C W, LIANG M, et al. Zearalenone exposure triggered cecal physical barrier injury through the TGF-β1/Smads signaling pathway in weaned piglets[J]. Toxins, 2021, 13(12):902.

[13]
DU H, JIANG D, SONG G, et al. Wound healing activity of phage-sisplayed TGF-β1 model peptide in streptozotocin-induced diabetic rats[J]. International Journal of Peptide Research and Therapeutics, 2021,27:1079-1094.

[14]
ROCHE J K, MARTINS C A, COSME R, et al. Transforming growth factor beta1 ameliorates intestinal epithelial barrier disruption by Cryptosporidium parvum in vitro in the absence of mucosal T lymphocytes[J]. Infection and Immunity, 2000, 68(10):5635-5644.

[15]
程群. 玉米赤霉烯酮诱导断奶仔猪肠道氧化应激及其机制的研究[D]. 硕士学位论文. 泰安: 山东农业大学, 2021.

CHENG Q. Study on intestinal oxidative stress induced by zearalenone in weaned piglets and its mechanism[D]. Master’s Thesis. Tai’an: Shandong Agricultural University, 2021.(in Chinese)

[16]
凌阿茹, 郭晋丽, 郭文博, 等. 玉米赤霉烯酮对蛋鸡生产性能、血液指标和生殖激素水平的影响[J]. 上海农业学报, 2019, 35(4):100-106.

LING A R, GUO J L, GUO W B, et al. Effects of zearalenone on laying performance,hematological indices and reproductive hormone levels in laying hens[J]. Acta Agriculturae Shanghai, 2019, 35(4):100-106.(in Chinese)

[17]
MOKOENA D, DHILIP KUMAR S S, HOURELD N N, et al. Role of photobiomodulation on the activation of the Smad pathway via TGF-β in wound healing[J]. Journal of Photochemistry and Photobiology B-Biology, 2018,189:138-144.

[18]
DERYNCK R, ZHANG Y. Smad-dependent and Smad-independent pathways in TGF-β family signalling[J]. Nature, 2003, 425(6958):577-584.

[19]
肖勘. TGF-β1在断奶仔猪肠上皮屏障损伤修复中的作用及其信号通路解析[D]. 硕士学位论文. 杭州: 浙江大学, 2017.

XIAO K. The role of TGF-β1 on intestinal epithelial barrier restoration and itssignal pathways in weaned piglets[D]. Master’s Thesis. Hangzhou: Zhejiang University, 2017.(in Chinese)

[20]
MASSAGUÉ J. The transforming growth factor-beta family[J]. Annual Review of Cell Biology, 1990,6:597-641.

[21]
MARTÍN-MATEOS R, ALBILLOS A. The role of the gut-liver axis in metabolic dysfunction-associated fatty liver disease[J]. Frontiers in Immunology, 2021,12:660179.

[22]
GU A X, YANG L G, WANG J J, et al. Protective effect of glutamine and alanyl-glutamine against zearalenone-induced intestinal epithelial barrier dysfunction in IPEC-J2 cells[J]. Research in Veterinary Science, 2021,137:48-55.

[23]
王玉, 郑春田, 温晓鹿, 等. 低聚壳聚糖对断奶仔猪生长性能及肠道健康的影响[C]//中国畜牧兽医学会动物营养学分会第十二次动物营养学术研讨会论文集.北京:中国农业大学出版社,2016:89.

WANGY, ZHENGC T, WENX L, et al. The effects of chitosan oligosaccharides on the growth performance and intestinal health of weaned piglets[C]//Proceedings of the 12th Academic Symposium on Animal Nutrition of the Animal Nutrition Branch of the Chinese Veterinary Medical Association. Beijing: China Agricultural University Press,2016:89.(in Chinese)

[24]
LIU Y M, YANG Y X, DONG R Q, et al. Protective effect of selenomethionine on intestinal injury induced by T-2 toxin[J]. Research in Veterinary Science, 2020,132:439-447.

[25]
SINGH P, WIG J D, SRINIVASAN R. The Smad family and its role in pancreatic cancer[J]. Indian Journal of Cancer, 2011, 48(3):351-360.

DOI PMID

[26]
YAN X H, CHEN Y G. SMAD7:not only a regulator, but also a cross-talk mediator of TGF-β signalling[J]. Biochemical Journal, 2011, 434(1):1-10.

[27]
张泆琳, 武鹏, 尹建新, 等. 圣草酚对TGF-β1诱导的人皮肤成纤维细胞增殖、氧化应激反应及TGF-β1/Smad信号通路活化的影响[J]. 广西医学, 2024, 46(6):873-881.

ZHANG Y L, WU P, YIN J X, et al. Effect of eriodictyol on proliferation,oxidative stress response and TGF-β1/Smad signaling pathway activation of human skin fibroblasts induced by TGF-β1[J]. Guangxi Medical Journal, 2024, 46(6):873-881.(in Chinese)

[28]
CARTHY J M. TGFβ signaling and the control of myofibroblast differentiation:implications for chronic inflammatory disorders[J]. Journal of Cellular Physiology, 2018, 233(1):98-106.

[29]
WU F Y, CUI J, YANG X Y, et al. Effects of zearalenone on genital organ development,serum immunoglobulin,antioxidant capacity,sex hormones and liver function of prepubertal gilts[J]. Toxicon, 2021,189:39-44.

[30]
王欢欢, 傅春妮, 李元辉, 等. 壳聚糖硒抗ZEA对仔猪肝肾抗氧化功能、血清E2含量和肝脏3β-HSD活性的影响[J]. 中国兽医杂志, 2021, 57(6):43-46,52.

WANG H H, FU C N, LI Y H, et al. Anti-zearalenone effects of chitosan selenium on hepatic and renal oxidative damage,serum E2 and 3β-HSD activity in weaning gilts[J]. Chinese Journal of Veterinary Medicine, 2021, 57(6):43-46,52.(in Chinese)

[31]
GU Y F, CHEN Y P, JIN R, et al. Dietary chitooligosaccharide supplementation alleviates intestinal barrier damage,and oxidative and immunological stress in lipopolysaccharide-challenged laying hens[J]. Poultry Science, 2022, 101(4):101701.

[32]
SANJABI S, OH S A, LI M O. Regulation of the immune response by TGF-β:from conception to autoimmunity and infection[J]. Cold Spring Harbor Perspectives in Biology, 2017, 9(6):a022236.

[33]
BATLLE E, MASSAGUÉ J. Transforming growth factor-β signaling in immunity and cancer[J]. Immunity, 2019, 50(4):924-940.

DOI PMID

[34]
DAVID C J, MASSAGUÉ J. Contextual determinants of TGFβ action in development,immunity and cancer[J]. Nature Reviews Molecular Cell Biology, 2018, 19(7):419-435.

[35]
DERYNCK R, TURLEY S J, AKHURST R J. TGFβ biology in cancer progression and immunotherapy[J]. Nature Reviews Clinical Oncology, 2021, 18(1):9-34.

[36]
MARIE J C, LIGGITT D, RUDENSKY A Y. Cellular mechanisms of fatal early-onset autoimmunity in mice with the T cell-specific targeting of transforming growth factor-beta receptor[J]. Immunity, 2006, 25(3):441-454.

DOI PMID

文章导航

/