研究论文

呕吐毒素对断奶仔猪脾脏和胸腺辅助性T细胞1/辅助性T细胞2和辅助性T细胞1/调节性T细胞稳态的影响

  • 徐先锋 , 1 ,
  • 李晓彤 1 ,
  • 刘凤玲 1 ,
  • 尉心田 1 ,
  • 舒奎 1 ,
  • 杨彩梅 2 ,
  • 肖勘 1 ,
  • 刘玉兰 1 ,
  • 陈少魁 , 1, *
展开
  • 1 武汉轻工大学动物科学与营养工程学院,动物营养与饲料科学湖北省重点实验室,武汉 430023
  • 2 浙江惠嘉生物科技股份有限公司,安吉 313307
*陈少魁,副教授,硕士生导师,E-mail:

徐先锋(1999—),男,湖北十堰人,硕士研究生,研究方向为猪营养与免疫研究。E-mail:

Copy editor: 武海龙

收稿日期: 2024-10-31

  网络出版日期: 2025-06-12

基金资助

国家自然科学基金面上项目(31772615)

Effects of Deoxynivalenol on T Helper Cells 1/T Helper Cells 2 and T Helper Cells 1/Regulatory T Cells Homeostasis in Spleen and Thymus of Weaned Piglets

  • XU Xianfeng , 1 ,
  • LI Xiaotong 1 ,
  • LIU Fengling 1 ,
  • YU Xintian 1 ,
  • SHU Kui 1 ,
  • YANG Caimei 2 ,
  • XIAO Kan 1 ,
  • LIU Yulan 1 ,
  • CHEN Shaokui , 1, *
Expand
  • 1 Hubei Key Laboratory of Animal Husbandry and Feed Science, College of Animal Science and Nutritional Engineering, Wuhan Polytechnic University, Wuhan 430023, China
  • 2 Zhejiang Huijia Biotechnology Co., Ltd., Anji 313307, China
* associate professor, E-mail:

Received date: 2024-10-31

  Online published: 2025-06-12

摘要

本试验旨在探究呕吐毒素(DON)对断奶仔猪脾脏和胸腺辅助性T细胞1(Th1)、辅助性T细胞2(Th2)和调节性T细胞(Treg)标志基因表达及Th1/Th2和Th1/Treg比例的影响。饲粮中添加DON试验:选取12头体重为(6.9±0.8) kg的28日龄“杜×长×大”三元杂交断奶仔猪,随机分为2组,每组6头猪。对照组(CON组)饲喂基础饲粮,DON组在基础饲粮中添加4 mg/kg DON。试验期21 d。静脉注射DON试验:选取12头体重为(7.3±0.4) kg的28日龄“杜×长×大”三元杂交断奶仔猪,随机分为2组,每组6头猪。CON组静脉注射生理盐水,DON组静脉注射0.8 mg/kg BW的DON。试验期6 h。结果表明:1)与CON组相比,饲粮中添加DON显著增加脾脏叉头框蛋白P3(FOXP3)的mRNA相对表达量(P<0.05),显著降低脾脏Th1/Treg比例(P<0.05);显著增加胸腺干扰素-γ(IFN-γ)和FOXP3的mRNA相对表达量(P<0.05),显著增加胸腺Th1/Th2比例(P<0.05)。2)与CON组相比,静脉注射DON显著增加脾脏IFN-γ、白细胞介素-6(IL-6)、GATA结合蛋白3(GATA3)、白细胞介素-4(IL-4)、FOXP3和白细胞介素-10(IL-10)的mRNA相对表达量(P<0.05),显著降低脾脏Th1/Th2比例(P<0.05);显著增加胸腺T-Box转录因子(T-bet)、FOXP3和IL-10的mRNA相对表达量(P<0.05),显著增加胸腺Th1/Th2比例(P<0.05)。由此可见,DON会引起脾脏和胸腺不同T细胞的变化,Th1/Th2和Th1/Treg比例失衡,造成断奶仔猪免疫功能紊乱。

本文引用格式

徐先锋 , 李晓彤 , 刘凤玲 , 尉心田 , 舒奎 , 杨彩梅 , 肖勘 , 刘玉兰 , 陈少魁 . 呕吐毒素对断奶仔猪脾脏和胸腺辅助性T细胞1/辅助性T细胞2和辅助性T细胞1/调节性T细胞稳态的影响[J]. 动物营养学报, 2025 , 37(6) : 3644 -3654 . DOI: 10.12418/CJAN2025.300

Abstract

The aim of this experiment was to investigate the effects of deoxynivalenol (DON) on the expression of T helper cells 1 (Th1), T helper cells 2 (Th2) and regulatory T cells (Treg) marker genes and Th1/Th2 and Th1/Treg ratios in spleen and thymus of weaned piglets. The dietary supplementation of DON experiment: twelve 28-day-old “Duroc×Landrace×Large White” three-way cross weaned piglets with body weight of (6.9±0.8) kg were randomly divided into two groups with 6 piglets per group. The control group (CON group) was fed a basal diet, and the DON group was fed the basal diet supplemented with 4 mg/kg DON. The experiment lasted for 21 days. The intravenous injection of DON experiment: twelve 28-day-old “Duroc×Landrace×Large White” three-way cross weaned piglets with body weight of (7.3±0.4) kg were randomly divided into two groups with 6 piglets per group. The CON group was injected intravenously with saline, and the DON group was injected intravenously with 0.8 mg/kg BW DON. The experiment lasted for 6 hours. The results showed as follows: 1) compared with the CON group, dietary supplementation of DON significantly increased the mRNA relative expression level of forkhead framing protein P3 (FOXP3) in spleen (P<0.05), and significantly decreased the Th1/Treg ratio in spleen (P<0.05); significantly increased the mRNA relative expression levels of interferon-γ (IFN-γ) and FOXP3 in thymus (P<0.05), and significant increase in the Th1/Th2 ratio in thymus (P<0.05). 2) Compared with the CON group, intravenous injection of DON significantly increased the mRNA relative expression levels of IFN-γ, interleukin-6 (IL-6), GATA binding protein 3 (GATA3), interleukin-4 (IL-4), FOXP3 and interleukin-10 (IL-10) in spleen (P<0.05), and significantly decreased the Th1/Th2 ratio in spleen (P<0.05); significantly increased the mRNA relative expression levels of T-Box transcription factor T-bet, FOXP3 and IL-10 in thymus (P<0.05), and significantly increased the Th1/Th2 ratio in thymus (P<0.05). In conclusion, DON induces the changes of different T cells in spleen and thymus, and the Th1/Th2 and Th1/Treg ratios are imbalance, causing immune dysfunction in weaned piglets.

呕吐毒素又名脱氧雪腐镰刀菌烯醇(deoxynivalenol,DON),是一种常见的霉菌毒素,广泛存在于小麦、大麦和玉米等谷物中[1-4]。研究发现,2018年至2020年间,我国不同地区饲料中DON的个体污染率超过96.4%[5]。猪是对DON最敏感的畜禽之一[6],猪群采食被霉菌毒素污染的饲料后,会出现多系统与多器官的病变、免疫功能降低、抗病力下降[7],诱发猪场疫情、种猪繁殖障碍、饲料利用率降低、生产性能下降等一系列问题,给养猪生产造成巨大的经济损失[8-9]
研究表明,免疫系统是DON的主要攻击对象[10-11],DON在被肠道吸收后会随着血液快速进入胸腺和脾脏等免疫器官[12],从而严重影响胸腺和脾脏对免疫系统正常功能的维持[13]。胸腺是T细胞发育和成熟的场所[14],脾脏是T细胞主要聚集和活化的场所[15]。成熟的T细胞从胸腺输出后,大量聚集于脾脏。成熟的T细胞包括CD4+辅助性T细胞和CD8+细胞毒性T细胞等,CD4+辅助性T细胞根据不同的分化途径和作用分为辅助性T细胞1(T helper cells 1,Th1)、辅助性T细胞2(T helper cells 2,Th2)与调节性T细胞(regulatory T cells,Treg)等亚群[16]。Pinton等[17]研究发现,DON对免疫系统的影响受其浓度、暴露时间和持续时间的影响。Wang等[18]研究发现,DON会通过改变仔猪淋巴细胞细胞因子mRNA水平从而影响淋巴细胞的免疫功能。多项研究发现,Th1/Th2和Th1/Treg比例的失衡会导致免疫功能紊乱,从而引发疾病[19-22]。然而,目前有关DON对仔猪Th1/Th2和Th1/Treg稳态影响的研究还很有限。
因此,本研究旨在通过在饲粮中添加或静脉注射DON建立仔猪DON慢性和急性损伤模型,探究DON对仔猪脾脏和胸腺Th1、Th2和Treg细胞标志基因表达及Th1/Th2和Th1/Treg稳态的影响,为缓解养猪生产中仔猪DON中毒提供新的方向。

1 材料与方法

1.1 试验材料

饲粮中添加的DON含量为587.5 mg/kg。DON具体培养过程为:将禾谷镰刀菌W3008株在马铃薯葡萄糖琼脂培养基上28 ℃下培养7 d以获得成熟孢子。将300 g玉米粉、50 g大米和140 mL无菌水加入1 L锥形瓶中,121 ℃高压灭菌20 min。每个烧瓶接种1×10⁶个/g禾谷镰刀菌孢子,在28 ℃和85%相对湿度下培养28 d后,将各烧瓶中霉菌污染的样品置于65 ℃烘箱中干燥过夜,混合,取样检测样品中DON含量。
静脉注射的DON纯度为99%。DON注射液配制方法为:将100 mg DON溶于生理盐水中,配制成10 mg/mL的母液,再将10 mg/mL的母液稀释成4 mg/mL的DON。注射剂量参照课题组前期试验及黄菲菲[23]的研究,按照0.8 mg/kg BW的剂量给仔猪静脉注射。

1.2 试验设计

饲粮中添加DON试验:选取12头体重(6.9±0.8) kg、健康、胎次接近的28日龄“杜×长×大”三元杂交断奶仔猪,随机分为2组,每组6头猪。对照组(CON组)饲喂基础饲粮,DON组在基础饲粮中添加4 mg/kg DON。饲喂21 d后,将仔猪麻醉屠宰,取脾脏和胸腺样品。
静脉注射DON试验:选取12头体重(7.3±0.4) kg、健康、胎次接近的28日龄“杜×长×大”三元杂交断奶仔猪,随机分为2组,每组6头猪。CON组静脉注射生理盐水;DON组静脉注射DON,注射剂量为0.8 mg/kg BW。注射6 h后,将仔猪麻醉屠宰,取脾脏和胸腺样品。

1.3 饲养管理

本试验在武汉轻工大学动物营养与饲料科学湖北省重点实验室进行。所有程序均经武汉轻工大学动物科学与营养工程学院动物护理与使用委员会批准(批准号:EM20221219008)。每个代谢笼(长×宽=1.80 m×1.10 m)中饲养1头仔猪,自由采食和饮水。动物房内温度控制在26~29 ℃。基础饲粮参照NRC(2012)仔猪营养需要量配制,其组成及营养水平见表1
表1 基础饲粮组成及营养水平(饲喂基础)

Table 1 Composition and nutrient levels of the basal diet (as-fed basis) %

项目Items 含量Content
原料Ingredients
玉米Corn 62.90
豆粕Soybean meal 7.50
发酵豆粕Fermented soybean meal 8.00
鱼粉Fish meal 5.00
低蛋白乳清粉Low protein whey powder 5.00
葡萄糖Glucose 2.00
豆油Soybean oil 5.00
磷酸氢钙CaHPO4 0.95
石粉Limestone 0.80
食盐NaCl 0.30
L-赖氨酸盐酸盐L-Lys·HCl (78%) 0.85
L-蛋氨酸L-Met (98%) 0.29
L-苏氨酸L-Thr (98%) 0.32
色氨酸Try 0.09
预混料Premix1) 1.00
合计Total 100.00
营养水平Nutrient levels2)
消化能DE/(MJ/kg) 14.75
粗蛋白质CP 17.47
钙Ca 0.81
总磷TP 0.62
总赖氨酸TLys 1.52
总蛋氨酸TMet 0.59
总蛋氨酸+总胱氨酸TMet+TCys 0.86
总苏氨酸TThr 0.93
总色氨酸TTry 0.26

1)预混料为每千克饲粮提供 The premix provided the following per kg of the diet:VA 5 512 IU,VB12 0.01 mg,VD3 2 200 IU,VE 30 IU,VK3 4 mg,核黄素 riboflavin 5.22 mg,D-泛酸钙 D-pantothenic acid calcium 20 mg,烟酸 nicotinic acid 26 mg,Mn (MnSO4·H2O) 40 mg,Fe (FeSO4·H2O) 75 mg,Zn (ZnSO4·7H2O) 75 mg,Cu (CuSO4·5H2O) 100 mg,I (CaI2) 0.3 mg,Se (Na2SeO3) 0.3 mg。
2)代谢能为计算值,其余为实测值。计算和测定方法参照王仁杰等[24]。ME was a calculated value, while the others were measured values. The calculation and measurement methods refer to Wang et al[24].

1.4 样品采集及处理

仔猪麻醉屠宰后,取脾脏和胸腺组织各一小块于4%多聚甲醛中进行固定,用于制作苏木精-伊红(HE)染色切片。剩余的脾脏、胸腺组织被切成小块,在液氮中快速冷冻,并储存在-80 ℃待测。

1.5 组织形态学观察

制作脾脏和胸腺HE染色切片及观察的具体步骤参照Ding等[13]的试验方法。

1.6 mRNA相对表达量测定

采用实时定量PCR方法检测脾脏和胸腺Th1、Th2和Treg细胞标志基因表达量。仔猪脾脏和胸腺RNA采用Trizol试剂(TaKaRa,日本),根据制造商的说明提取。用逆转录试剂盒(TaKaRa,日本)将RNA定量并转录成cDNA,测定的具体方法参照秦旭等[25]。引物序列如表2所示。内参基因为β-肌动蛋白(β-actin),目的基因包括T-Box转录因子(T-bet)、干扰素-γ(IFN-γ)、白细胞介素-6(IL-6)、肿瘤坏死因子-α(TNF-α)、GATA结合蛋白3(GATA3)、白细胞介素-4(IL-4)、叉头框蛋白P3(FOXP3)、白细胞介素-10(IL-10),目的基因mRNA相对表达量的计算方法参照Livak等[26]
表2 引物序列

Table 2 Primer sequences

基因
Genes
引物序列
Primer sequences (5'—3')
登录号
Accession number
产物大小
Product size/bp
T-Box转录因子
T-bet
F:TCCTCGGAGCCTATGCCTAC
R:GAATGGGAACATCCGCCGTC
NM_001315722.1 296
干扰素-γ
IFN-γ
F:TTCCAAGGCCAGAGAGCATC
R:TACCTAGTTGGCCCCTGAGA
XM_047787150.1 294
白细胞介素-6
IL-6
F:AAGGTGATGCCACCTCAGAC
R:TCTGCCAGTACCTCCTTGCT
JQ839263.1 151
肿瘤坏死因子-α
TNF-α
F:AAGACACCATGAGCACTGAGA
R:CGACCAGGAGGAAGGAGAAG
JF831365.1 132
GATA结合蛋白3
GATA3
F:CGAGGTCCAGCACAGAAGG
R:AGCCTTCGCTTGGGCTTAAT
NM_001044567.1 160
白细胞介素-4
IL-4
F:CTCCCAACTGATCCCAACCC
R:TGCACGAGTTCTTTCTCGCT
NM_214123.1 134
叉头框蛋白P3
FOXP3
F:TCCACTTCACCAAGCCTGC
R:GCATGGGGTTCAAGGAGGAA
NM_001128438.1 229
白细胞介素-10
IL-10
F:CCACAAGTCCGACTCAACGA
R:GGCAACCCAGGTAACCCTTA
NM_214041.1 267
β-肌动蛋白
β-actin
F:TGCGGGACATCAAGGAGAAG
R:AGTTGAAGGTGGTCTCGTGG
AF017079.1 194

1.7 统计分析

采用Graphpad Prism 9.5软件进行统计学检验。Th1、Th2和Treg细胞标志基因mRNA相对表达量在2组之间的比较均采用独立样本t检验。P<0.05为差异显著,0.05<P<0.10为有差异显著趋势。

2 结果

2.1 饲料中添加DON对仔猪脾脏和胸腺形态结构的影响

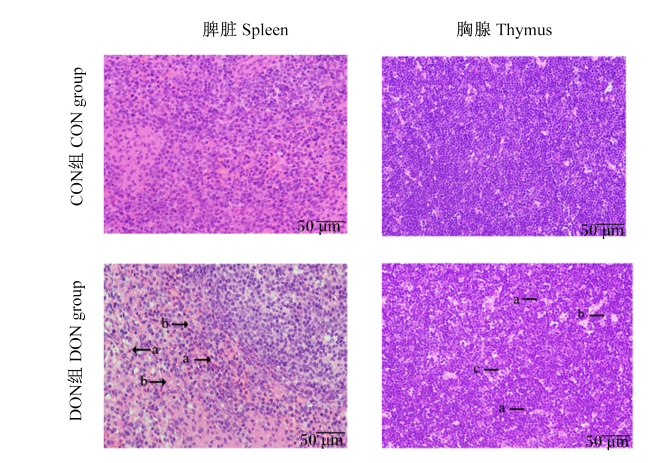
图1所示,与CON组相比,DON组脾脏出现炎性细胞浸润、白髓充血;胸腺出现坏死细胞,有大量的网状化细胞和纤维化细胞。
图1 饲料中添加DON对仔猪脾脏和胸腺形态结构的影响

脾脏:(a)炎性细胞浸润,(b)白髓充血;胸腺:(a)成纤维细胞,(b)大量网状细胞,(c)少量坏死细胞。

Fig.1 Effects of dietary supplementation of DON on spleen and thymus morphology of piglets (400×)

Spleen: (a) inflammatory cell infiltration, (b) white pulp congestion; thymus: (a) fibroblasts, (b) a large number of reticular cells, (c) a small number of necrotic cells.

2.2 饲料中添加DON对仔猪脾脏Th1、Th2和Treg标志基因表达以及Th1/Th2和Th1/Treg比例的影响
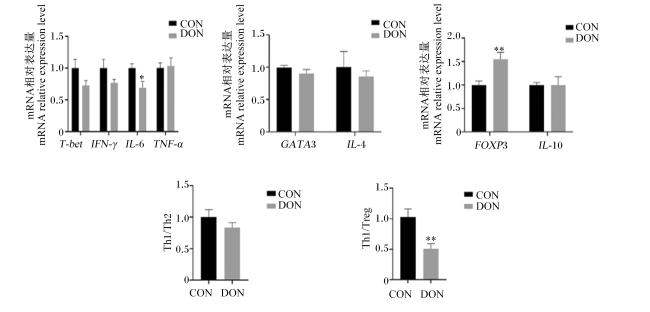
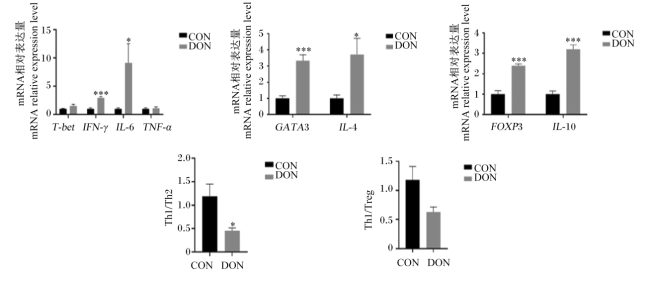
图2所示,与CON组相比,DON组脾脏IL-6的mRNA相对表达量显著降低(P<0.05),脾脏FOXP3的mRNA相对表达量显著升高(P<0.05),脾脏Th1/Treg比例显著降低(P<0.05)。
图2 饲料中添加DON对仔猪脾脏Th1、Th2和Treg标志基因表达以及Th1/Th2和Th1/Treg比例的影响
CON:CON组 CON group;DON:DON组 DON group;T-bet:T-Box转录因子 T-Box transcription factor;IFN-γ:干扰素-γ interferon-γ;IL-6:白细胞介素-6 interleukin-6;TNF-α:肿瘤坏死因子-α tumor necrosis factor-α;GATA3:GATA结合蛋白3 GATA binding protein 3;IL-4:白细胞介素-4 interleukin-4;FOXP3:叉头框蛋白P3;forkhead framing protein P3:IL-10:白细胞介素-10 interleukin-10;Th1/Th2:辅助性T细胞1/辅助性T细胞2比例 T helper cells 1/ T helper cells 2 ratio;Th1/Treg;辅助性T细胞1/调节性T细胞比例 T helper cells 1/regulatory T cells ratio。下图同 the same as below。

*、**、***均表示差异显著(P<0.05)。下图同。

Fig.2 Effects of dietary supplementation of DON on expression of Th1, Th2 and Treg marker genes and Th1/Th2 and Th1/Treg ratios in spleen of piglets

*, ** and *** all indicated significant difference (P<0.05). The same as below.

2.3 饲料中添加DON对仔猪胸腺Th1、Th2和Treg标志基因表达以及Th1/Th2和Th1/Treg比例的影响

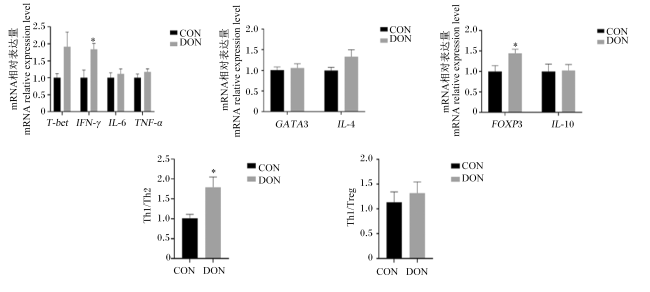
图3所示,与CON组相比,DON组胸腺IFN-γFOXP3的mRNA相对表达量显著升高(P<0.05),胸腺T-bet的mRNA相对表达量有升高趋势(P=0.071),脾脏的Th1/Th2比例显著升高(P<0.05)。
图3 饲料中添加DON对仔猪胸腺Th1、Th2和Treg标志基因表达以及Th1/Th2和Th1/Treg比例的影响

Fig.3 Effects of dietary supplementation of DON on expression of Th1, Th2 and Treg marker genes and Th1/Th2 and Th1/Treg ratios in thymus of piglets

2.4 静脉注射DON对仔猪脾脏和胸腺形态结构的影响

图4所示,与CON组相比,DON组脾脏组织出现网状化、空泡化及核固缩,还可见细胞发生坏死;胸腺细胞大量坏死,具体表现为出现空泡化和网状化细胞,同时伴随炎性渗出。
图4 静脉注射DON对仔猪脾脏和胸腺形态结构的影响

脾脏:(a)核固缩,(b)细胞网状化,(c)细胞空泡化;胸腺:(a)炎性渗出,(b)网状细胞,(c)细胞空泡化。

Fig.4 Effects of intravenous injection of DON on spleen and thymus morphology of piglets (400×)

Spleen: (a) nuclear condensation, (b) cellular reticular formation, (c) cellular vacuolization; thymus: (a) inflammatory exudation, (b) reticular cells, (c) cellular vacuolization.

2.5 静脉注射DON对仔猪脾脏Th1、Th2和Treg标志基因表达以及Th1/Th2和Th1/Treg比例的影响

图5所示,与CON组相比,DON组脾脏IFN-γIL-6、GATA3、IL-4、FOXP3、IL-10的mRNA相对表达量显著升高(P<0.05),脾脏Th1/Th2比例显著降低(P<0.05),Th1/Treg比例有下降趋势(P=0.072)。
图5 静脉注射DON对仔猪脾脏Th1、Th2和Treg标志基因表达以及Th1/Th2和Th1/Treg比例的影响

Fig.5 Effects of intravenous injection of DON on expression of Th1, Th2 and Treg marker genes and Th1/Th2 and Th1/Treg ratios in spleen of piglets

2.6 静脉注射DON对仔猪胸腺Th1、Th2和Treg标志基因表达以及Th1/Th2和Th1/Treg比例的影响

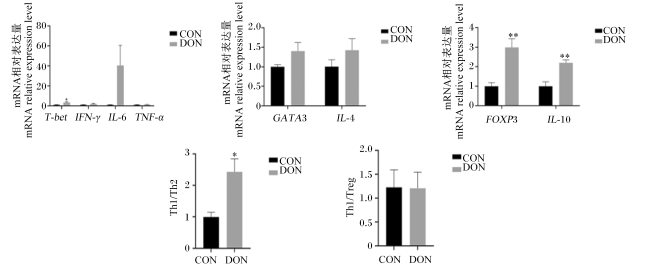
图6所示,与CON组相比,DON组胸腺T-betFOXP3和IL-10的mRNA相对表达量显著升高(P<0.05),胸腺IL-6的mRNA相对表达量有升高趋势(P=0.064),胸腺Th1/Th2比例显著升高(P<0.05)。
图6 静脉注射DON对仔猪胸腺Th1、Th2和Treg标志基因表达以及Th1/Th2和Th1/Treg比例的影响

Fig.6 Effects of intravenous injection of DON on expression of Th1, Th2 and Treg marker genes and Th1/Th2 and Th1/Treg ratios in thymus of piglets

3 讨论

DON作为广泛存在于饲料中的霉菌毒素之一,其化学性能非常稳定,一般不会在加工和储存过程中破坏,而现有的技术难以将其完全去除,在饲料中有较高残留[27];而猪的免疫系统对DON十分敏感,该毒素导致的免疫异常对猪的生长发育造成了不可忽略的影响[28],所以本试验重点探究DON对仔猪脾脏和胸腺的影响,为后续开展的营养调控缓解DON造成的免疫系统损伤建立基础。
研究发现,脾脏和胸腺是DON介导毒素的主要靶器官,程群等[29]研究发现,DON显著影响断奶仔猪血清和脾脏抗氧化能力,并通过改变脾脏白细胞介素-1β(IL-1β)和IL-6的表达和分布,降低脾脏的免疫功能;同时,DON会在断奶仔猪中引起胸腺组织病变,导致胸腺皮质淋巴细胞坏死,破坏氧化-抗氧化系统平衡,最终导致促炎因子IL-6、TNF-α的mRNA相对表达量升高[6,12,30]。在本试验中,通过在饲粮中添加DON建立慢性DON模型,饲粮中添加的DON需要通过消化道吸收和代谢后才能进入血液循环系统,其需要较长时间才能达到高峰,见效较慢,但持续时间长,可以更好地模拟生产过程中猪长期摄入霉变饲料后脾脏和胸腺的变化情况;而通过给仔猪静脉注射DON建立急性DON模型,DON则可以直接通过血液循环系统较快地分布到全身各个组织,静脉注射剂量大,可以更快地到达高峰,可能更容易引起全身性的炎症反应,有利于更好更快地探究DON对仔猪脾脏和胸腺的影响。本研究结果显示,在饲粮中添加DON和静脉注射DON可增加仔猪脾脏、胸腺中促炎细胞因子IL-6、IFN-γ的mRNA相对表达量。由此可见,DON会造成脾脏和胸腺损伤,导致炎症发生,从而降低仔猪的免疫功能。不仅如此,DON还会上调IL-10的表达,众所周知,促炎和抗炎因子之间的失衡会导致免疫失调,当平衡偏向抗炎因子时,将诱导免疫抑制[31]。在本试验中,静脉注射DON显著增加仔猪脾脏和胸腺中抗炎细胞因子IL-10的mRNA相对表达量,但在饲粮中添加DON对脾脏和胸腺中IL-10的mRNA相对表达量无显著影响。这些差异可能是由于DON的剂量、作用方式及时间不同所导致的。这也说明高剂量DON会抑制仔猪的免疫功能。因此,深入研究DON对脾脏和胸腺的损伤机制为预防DON对猪免疫功能的危害提供重要理论基础。
Rajput等[32]研究发现,DON会降低胸腺CD4+ T细胞百分比。Ren等[33]研究发现,小鼠腹腔注射DON后,血液中CD3+、CD4+ T细胞数量显著下降。这说明DON会干扰T细胞的分化,而CD4+ T细胞可以分化为Th1、Th2和Treg,因此本试验检测了仔猪受到DON刺激后脾脏和胸腺中CD4+ T细胞的亚群变化情况。Th1主要产生IFN-γ、IL-6和TNF-α等促炎因子,转录因子T-bet是Th1的特异性转录因子;Th2主要产生IL-4和白细胞介素-5(IL-5)等抗炎因子,GATA3是Th2细胞的特异性转录因子;Treg主要产生IL-10和转化生长因子-β(TGF-β)等抗炎因子,FOXP3是Treg细胞的特异性转录因子。大量研究结果表明,这些特异性核转录因子调控并维持相应辅助性T细胞亚型的分化和功能,因此通过检测这些转录因子的表达可以定量分析不同辅助性T细胞亚群在免疫反应中的变化,有助于评估机体免疫状态的变化[34-36]。Th1/Th2和Th1/Treg比例的失衡会导致免疫功能紊乱,引发多种免疫性疾病[21]。Th1/Th2和Th1/Treg比例上升通常表示机体细胞免疫功能增强,Th1细胞活性增加,可能是由于某种病原体感染或自身免疫性疾病的发生;Th1/Th2比例下降通常表示机体体液免疫功能增强,Th2细胞活性增加,可能是由于寄生虫感染、过敏反应等;Th1/Treg比例下降通常表示机体处于免疫抑制或免疫耐受状态,Treg的免疫抑制作用增强,可能是由于持续的抗原刺激导致。Becker等[37]研究发现,饲喂含有DON的玉米可增加猪的Th1数量;另有研究表明,DON处理增加了肠道呼肠孤病毒感染的小鼠肠系膜淋巴结中IL-4和IL-10的mRNA相对表达量,增强了Th2细胞因子的表达[38]。本试验结果显示,静脉注射DON显著上调仔猪脾脏中Th1分泌细胞因子IFN-γ、Th2核转录因子GATA3和分泌细胞因子IL-4的表达,然而Th2的变化比Th1更为明显,使Th1/Th2比例显著下降;而在胸腺中,无论是在饲粮中添加DON还是静脉注射DON,都会使Th1核转录因子T-bet的表达上调,Th2核转录因子和分泌细胞因子无明显变化,导致Th1/Th2比例显著上升,这与Jia等[39]的研究结果一致,即DON通过上调T细胞中T-bet的表达抑制Th2的分化,导致Th1/Th2比例失衡,从而引发机体免疫功能紊乱,这是DON引起胸腺炎症的重要机制之一。Treg作为维持机体免疫耐受与免疫平衡的主要功能细胞,它与Th1的平衡同样对机体免疫功能的影响至关重要[40],当Treg过度表达可导致免疫抑制[41]。本试验发现,在饲粮中添加DON或静脉注射DON都会使脾脏和胸腺中的Treg核转录因子FOXP3表达显著上调,降低脾脏中Th1/Treg比例,这说明Th1/Treg的稳态也在DON导致的免疫功能紊乱中发挥作用。

4 结论

饲粮中添加DON或静脉注射DON引起了仔猪脾脏和胸腺组织损伤,同时还引起了炎性细胞因子、Th1、Th2和Treg的特异性核转录因子和分泌细胞因子基因表达的改变,导致了仔猪脾脏和胸腺中Th1/Th2和Th1/Treg比例失衡。
[1]
侯然然, 张敏红. 霉菌毒素对畜禽的危害及其防控方法的研究进展[J]. 中国畜牧兽医, 2007, 34(1):13-16.

HOU R R, ZHANG M H. Damage of mycotoxins on animals and advances in study on methods of revention[J]. China Animal Husbandry & Veterinary Medicine, 2007, 34(1):13-16.(in Chinese)

[2]
肖长峰, 朱明芬, 潘雪男, 等. 霉菌毒素对畜牧业的危害及其防治措施[J]. 饲料工业, 2014, 35(22):62-65.

XIAO C F, ZHU M F, PAN X N, et al. Damage of mycotoxins on animal husbandry and its prevention and control measures[J]. Feed Industry, 2014, 35(22):62-65.(in Chinese)

[3]
曹宇, 党萌, 王明阳, 等. 饲料中呕吐毒素的危害和生物脱毒方法研究进展[J]. 中国猪业, 2017, 12(6):40-45.

CAO Y, DANG M, WANG M Y, et al. Research progress on the harm of vomiting toxin and biological detoxification methods in feed[J]. China Swine Industry, 2017, 12(6):40-45.(in Chinese)

[4]
王晓林. 霉菌毒素对养猪业的危害[J]. 中国猪业, 2017, 12(10):41-45.

WANG X L. Damage of mycotoxins on pig husbandry[J]. China Swine Industry, 2017, 12(10):41-45.(in Chinese)

[5]
ZHAO L, ZHANG L, XU Z J, et al. Occurrence of aflatoxin B1,deoxynivalenol and zearalenone in feeds in China during 2018-2020[J]. Journal of Animal Science and Biotechnology, 2021, 12(1):74.

[6]
MIKAMI O, YAMAGUCHI H, MURATA H, et al. Induction of apoptotic lesions in liver and lymphoid tissues and modulation of cytokine mRNA expression by acute exposure to deoxynivalenol in piglets[J]. Journal of Veterinary Science, 2010, 11(2):107-113.

PMID

[7]
PIERRON A, ALASSANE-KPEMBI I, OSWALD I P. Impact of mycotoxin on immune response and consequences for pig health[J]. Animal Nutrition, 2016, 2(2):63-68.

DOI PMID

[8]
GAUTHIER T, WACHÉ Y, LAFFITTE J, et al. Deoxynivalenol impairs the immune functions of neutrophils[J]. Molecular Nutrition & Food Research, 2013, 57(6):1026-1036.

[9]
GAB-ALLAH M A, CHOI K, KIM B. Type B trichothecenes in cereal grains and their products:recent advances on occurrence,toxicology,analysis and post-harvest decontamination strategies[J]. Toxins, 2023, 15(2):85.

[10]
MISHRA S, SRIVASTAVA S, DEWANGAN J, et al. Global occurrence of deoxynivalenol in food commodities and exposure risk assessment in humans in the last decade:a survey[J]. Critical Reviews in Food Science and Nutrition, 2020, 60(8):1346-1374.

[11]
LIAO Y X, PENG Z, CHEN L K, et al. Deoxynivalenol,gut microbiota and immunotoxicity:a potential approach?[J]. Food and Chemical Toxicology, 2018,112:342-354.

[12]
ZHANG L, MA R, ZHU M X, et al. Effect of deoxynivalenol on the porcine acquired immune response and potential remediation by a novel modified HSCAS adsorbent[J]. Food and Chemical Toxicology, 2020,138:111187.

[13]
DING D J, MOU D L, ZHAO L P, et al. Maternal organic selenium supplementation alleviates LPS induced inflammation,autophagy and ER stress in the thymus and spleen of offspring piglets by improving the expression of selenoproteins[J]. Food & Function, 2021, 12(22):11214-11228.

[14]
DUAH M, LI L L, SHEN J Y, et al. Thymus degeneration and regeneration[J]. Frontiers in Immunology, 2021,12:706244.

[15]
LEWIS S M, WILLIAMS A, EISENBARTH S C. Structure and function of the immune system in the spleen[J]. Science Immunology, 2019, 4(33):eaau6085.

[16]
HUO Y F, FENG Q, FAN J, et al. Serum brain-derived neurotrophic factor in coronary heart disease:correlation with the T helper (Th) 1/Th2 ratio,Th17/regulatory T (Treg) ratio,and major adverse cardiovascular events[J]. Journal of Clinical Laboratory Analysis, 2023, 37(1):e24803.

[17]
PINTON P, BRAICU C, NOUGAYREDE J P, et al. Deoxynivalenol impairs porcine intestinal barrier function and decreases the protein expression of claudin-4 through a mitogen-activated protein kinase-dependent mechanism[J]. The Journal of Nutrition, 2010, 140(11):1956-1962.

[18]
WANG X M, ZUO Z C, DENG J L, et al. Protective role of selenium in immune-relevant cytokine and immunoglobulin production by piglet splenic lymphocytes exposed to deoxynivalenol[J]. Biological Trace Element Research, 2018, 184(1):83-91.

DOI PMID

[19]
HARAKAL J, RIVAL C, QIAO H, et al. Regulatory T cells control Th2-dominant murine autoimmune gastritis[J]. Journal of Immunology, 2016, 197(1):27-41.

DOI PMID

[20]
MOHAMMADI S V, REZAEI A, ANDALIB A, et al. Improvement of Th1/Th2 and Th1/Treg imbalances by adjutants CPG,MPLA and BCG in a model of acute asthma induced by allergen Derp2 in BALB/c mice[J]. Iranian Red Crescent Medical Journal, 2017, 19(3):e41114.

[21]
ZHANG Y, ZHANG Y G, GU W P, et al. Th1/Th2 cell’s function in immune system[J]. Advances in Experimental Medicine and Biology, 2014,841:45-65.

[22]
NIE Z Q, HAN D, ZHANG K, et al. Th1/Treg ratio may be a marker of autism in children with immune dysfunction[J]. Research in Autism Spectrum Disorders, 2023,101:102085.

[23]
黄菲菲. 线粒体分裂融合失衡在呕吐毒素诱导的仔猪肠道损伤中的作用[D]. 硕士学位论文. 武汉: 武汉轻工大学, 2022.

HUANG F F. The role of mitochondrial fission and fusion imbalance in deoxynivalenol-induced porcine intestinal injury[D]. Master’s Thesis. Wuhan: Wuhan Polytechnic University, 2022.(in Chinese)

[24]
王仁杰, 宋孝明, 谢实勇, 等. 棉籽浓缩蛋白替代发酵豆粕对仔猪生长性能、营养物质消化率、血液指标和粪便微生物代谢的影响[J]. 中国饲料, 2023(22):211-219.

WANG R J, SONG X M, XIE S Y, et al. Effects of cottonseed protein concentrate to replace fermented soybean meal on growth performance,nutrient digestibility,blood indices and fecal microbiota metabolism of weaned pig[J]. China Feed, 2023(22):211-219.(in Chinese)

[25]
秦旭, 周墨涵, 尉心田, 等. 脂多糖刺激后不同时间点断奶仔猪肠道中凋亡和自噬信号通路的动态变化[J]. 动物营养学报, 2023, 35(3):1513-1519.

DOI

QIN X, ZHOU M H, WEI X T, et al. Dynamic change of apoptosis and autophagy signal pathways in intestinal tract of weaned piglets after lipopolysaccharide challenge at different time points[J]. Chinese Journal of Animal Nutrition, 2023, 35(3):1513-1519.(in Chinese)

DOI

[26]
LIVAK K J, SCHMITTGEN T D. Analysis of relative gene expression data using real-time quantitative PCR and the 2-ΔΔCT method[J]. Methods, 2001, 25(4):402-408.

[27]
REN Z H, GUO C Y, HE H Y, et al. Effects of deoxynivalenol on mitochondrial dynamics and autophagy in pig spleen lymphocytes[J]. Food and Chemical Toxicology, 2020,140:111357.

[28]
HOOFT J M, BUREAU D P. Deoxynivalenol: Mechanisms of action and its effects on various terrestrial and aquatic species[J]. Food and Chemical Toxicology, 2021,157:112616.

[29]
程群, 姜淑贞, 陈宁波, 等. 镰刀菌毒素对断奶仔猪脾脏抗氧化能力和白细胞介素-1β、白细胞介素-6分布和表达的影响[J]. 动物营养学报, 2017, 29(9):3267-3276.

CHENG Q, JIANG S Z, CHEN N B, et al. Effects of fusarium toxins on antioxidant capacity and distribution and expression of interleukin-1β and interleukin-6 in spleen of weaned piglets[J]. Chinese Journal of Animal Nutrition, 2017, 29(9):3267-3276.(in Chinese)

[30]
AMUZIE C J, HARKEMA J R, PESTKA J J. Tissue distribution and proinflammatory cytokine induction by the trichothecene deoxynivalenol in the mouse:comparison of nasal vs.oral exposure[J]. Toxicology, 2008, 248(1):39-44.

[31]
王晴. DON对PEDV感染仔猪免疫功能的影响及其机理研究[D]. 硕士学位论文. 南京: 南京农业大学, 2021.

WANG Q. Effects of DON on the immune function of PEDV-infected piglets and its mechanism[D]. Master’s Thesis. Nanjing: Nanjing Agricultural University, 2021.(in Chinese)

[32]
RAJPUT S A, SHAUKAT A, RAJPUT I R, et al. Ginsenoside Rb1 prevents deoxynivalenol-induced immune injury via alleviating oxidative stress and apoptosis in mice[J]. Ecotoxicology and Environmental Safety, 2021,220:112333.

[33]
REN Z H, DENG H D, WANG Y C, et al. The fusarium toxin zearalenone and deoxynivalenol affect murine splenic antioxidant functions,interferon levels,and T-cell subsets[J]. Environmental Toxicology and Pharmacology, 2016,41:195-200.

[34]
SZABO S J, KIM S T, COSTA G L, et al. A novel transcription factor,T-bet,directs Th1 lineage commitment[J]. Cell, 2000, 100(6):655-669.

[35]
ZHENG W, FLAVELL R A. The transcription factor GATA-3 is necessary and sufficient for Th2 cytokine gene expression in CD4 T cells[J]. Cell, 1997, 89(4):587-596.

DOI PMID

[36]
FONTENOT J D, GAVIN M A, RUDENSKY A Y. Foxp3 programs the development and function of CD4+CD25+ regulatory T cells[J]. Nature Immunology, 2003, 4(4):330-336.

[37]
BECKER, B A, PACE, et al. Effects of feeding graded concentrations of Fusarium proliferatum culture material,containing known amounts of fumonisin B1,on swine growth and health[J]. Veterinary and Human Toxicology, 1997, 39(2):96-100.

[38]
LI M X, CUFF C F, PESTKA J. Modulation of murine host response to enteric reovirus infection by the trichothecene deoxynivalenol[J]. Toxicological Sciences, 2005, 87(1):134-145.

PMID

[39]
JIA L, SHI Y, WEN Y, et al. The role of T-bet as a central mediator for lineage commitment of CD4+T cells[J]. Journal of Leukocyte Biology, 2014, 95(5):699-701.

[40]
方伟. 孟鲁司特治疗对支气管哮喘患者肺功能及Th1、Treg平衡的调节作用[J]. 数理医药学杂志, 2021, 34(9):1368-1370.

FANG W. Regulation of menluster treatment on lung function and Th1,Treg balance in patients with bronchial asthma[J]. Journal of Mathematical Medicine, 2021, 34(9):1368-1370.(in Chinese)

[41]
郭琦, 薛鹏, 尹恒山, 等. 口腔癌前病损转化微环境中IL-1β/Treg、Th17/Treg、Th1/Th2免疫失衡的机制研究[J]. 实用癌症杂志, 2023, 38(5):775-778.

GUO Q, XUE P, YIN H S, et al. Mechanisms of immune imbalances of IL-1β/Treg, Th17/Treg and Th1/Th2 in the transformed microenvironment of oral precancerous lesions[J]. The Practical Journal of Cancer, 2023, 38(5):775-778.(in Chinese)

文章导航

/