

1 材料与方法
1.1 试验材料
1.2 试验设计和饲粮
表1 饲粮组成及营养水平(干物质基础)Table 1 Composition and nutrient levels of diets (DM basis)% |
| 项目 Items | 粗饲料来源 Roughage sources | ||||||||||
|---|---|---|---|---|---|---|---|---|---|---|---|
| 黑麦草 Ryegrass | 黑麦草青贮 Ryegrass silage | 葵花头 Sunflower head | 葵花头青贮 Sunflower head silage | 芦苇草 Alfa | 芦苇草青贮 Alfa silage | 3年生柠条 Three-year caragana | 3年生 柠条青贮 Three-year caragana silage | 燕麦草 Oat grass | 燕麦草青贮 Oat grass silage | ||
| 原料 Ingredients | |||||||||||
| 粗饲料 Roughage | 60.00 | 60.00 | 60.00 | 60.00 | 60.00 | 60.00 | 60.00 | 60.00 | 60.00 | 60.00 | |
| 玉米 Corn | 19.54 | 19.54 | 19.54 | 19.54 | 19.54 | 19.54 | 19.54 | 19.54 | 19.54 | 19.54 | |
| 豆粕 Soybean meal | 5.95 | 5.95 | 5.95 | 5.95 | 5.95 | 5.95 | 5.95 | 5.95 | 5.95 | 5.95 | |
| 麸皮 Bran | 2.99 | 2.99 | 2.99 | 2.99 | 2.99 | 2.99 | 2.99 | 2.99 | 2.99 | 2.99 | |
| 干酒糟及其可溶物 DDGS | 7.82 | 7.82 | 7.82 | 7.82 | 7.82 | 7.82 | 7.82 | 7.82 | 7.82 | 7.82 | |
| 食盐 NaCl | 0.87 | 0.87 | 0.87 | 0.87 | 0.87 | 0.87 | 0.87 | 0.87 | 0.87 | 0.87 | |
| 石粉 Limestone | 0.29 | 0.29 | 0.29 | 0.29 | 0.29 | 0.29 | 0.29 | 0.29 | 0.29 | 0.29 | |
| 预混料 Premix1) | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | |
| 磷酸氢钙 CaHPO4 | 0.60 | 0.60 | 0.60 | 0.60 | 0.60 | 0.60 | 0.60 | 0.60 | 0.60 | 0.60 | |
| 小苏打 NaHCO3 | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | 0.97 | |
| 合计 Total | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | |
| 营养水平 Nutrient levels2) | |||||||||||
| 代谢能ME/(MJ/kg) | 11.02 | 11.35 | 11.18 | 11.25 | 11.36 | 11.31 | 11.24 | 11.22 | 11.23 | 11.25 | |
| 粗蛋白质 CP | 11.23 | 11.57 | 12.22 | 12.29 | 11.08 | 11.00 | 12.01 | 12.25 | 11.44 | 11.52 | |
| 钙 Ca | 0.54 | 0.52 | 0.65 | 0.64 | 0.48 | 0.47 | 0.68 | 0.66 | 0.87 | 0.88 | |
| 磷 P | 0.32 | 0.33 | 0.31 | 0.30 | 0.30 | 0.33 | 0.31 | 0.35 | 0.34 | 0.38 | |
| 中性洗涤纤维NDF | 54.40 | 47.06 | 49.69 | 52.89 | 47.69 | 53.78 | 45.12 | 45.91 | 54.71 | 50.41 | |
| 粗灰分 Ash | 5.58 | 5.24 | 5.17 | 6.50 | 9.15 | 9.59 | 4.69 | 4.97 | 6.52 | 5.59 | |
| 酸性洗涤纤维ADF | 31.79 | 32.49 | 34.91 | 33.72 | 29.54 | 28.52 | 30.50 | 30.27 | 41.43 | 40.08 | |
| 粗脂肪 EE | 6.79 | 6.82 | 7.16 | 7.21 | 6.17 | 6.26 | 7.65 | 7.70 | 5.77 | 5.69 | |
1)每千克预混料含有 Each kilogram of the premix contained:VA 150 000 IU,VD2 20 000 IU,VE 175 IU,Fe 1 000~1 500 mg,Mn 300~600 mg,Zn 600~1 000 mg,Cu 80~200 mg,I 6~12 mg,Se 4~6 mg,Co 3~5 mg,Ca 150~200 g,NaCl 100~250 g。 |
1.3 测定指标及方法
1.3.1 饲粮及原料样品营养成分含量
1.3.2 CNCPS组分
1.3.3 瘤胃菌群
1.4 数据统计分析
2 结果与分析
2.1 不同粗饲料CNCPS蛋白质组分
表2 不同粗饲料CNCPS蛋白质组分(干物质基础)Table 2 CNCPS protein components of different roughages (DM basis)% CP |
| 项目 Items | 非蛋白氮 PA | 快速降解蛋白 PB1 | 中速降解蛋白 PB2 | 慢速降解蛋白 PB3 | 不可利用氮 PC |
|---|---|---|---|---|---|
| 黑麦草 Ryegrass | 30.81±1.71c | 11.12±0.59e | 6.28±0.88cd | 6.00±0.13d | 23.61±0.78cd |
| 黑麦草青贮 Ryegrass silage | 28.21±1.66c | 12.56±3.75e | 7.42±0.41bc | 6.41±0.24d | 22.43±1.14d |
| 葵花头 Sunflower head | 29.69±3.02c | 22.87±0.56bc | 7.28±0.12bc | 3.70±0.74ef | 25.78±0.41bc |
| 葵花头青贮 Sunflower head silage | 27.88±0.45c | 20.26±1.69d | 7.64±0.21b | 2.32±1.32g | 24.46±1.26bcd |
| 芦苇草 Alfa | 22.93±0.13d | 17.43±0.08d | 10.33±0.16a | 10.36±0.12b | 27.97±0.25ab |
| 芦苇草青贮 Alfa silage | 21.17±1.11d | 23.56±2.56b | 9.98±0.01a | 8.20±0.10c | 28.69±0.39a |
| 3年生柠条 Three-year caragana | 54.30±2.38a | 33.72±2.11a | 5.61±0.73d | 4.75±0.43e | 23.11±2.06cd |
| 3年生柠条青贮 Three-year caragana silage | 53.00±0.32a | 34.97±4.25a | 5.60±0.64d | 3.12±0.51f | 27.61±0.70ab |
| 燕麦草 Oat grass | 36.64±2.93b | 20.79±1.39cd | 7.68±0.66b | 19.37±1.00a | 24.54±1.17bcd |
| 燕麦草青贮 Oat grass silage | 29.72±0.66c | 21.84±0.99bc | 8.28±0.92b | 19.87±1.25a | 26.30±2.43bc |
2.2 不同粗饲料CNCPS CHO组分
表3 不同粗饲料CNCPS CHO组分(干物质基础)Table 3 CNCPS CHO components of different roughages (DM basis) |
| 项目 Items | 碳水化合物 CHO/% DM | 非结构性 碳水化合物 NSC/% CHO | 快速降解 碳水化合物 CA/% CHO | 中速降解 碳水化合物 CB1/% CHO | 慢速降解 碳水化合物 CB2/% CHO | 不可利用 碳水化合物 CC/% CHO |
|---|---|---|---|---|---|---|
| 黑麦草 Ryegrass | 80.57±0.42b | 15.05±0.51e | 20.16±4.39bc | 12.11±0.20bc | 62.37±6.21bcd | 14.36±0.27f |
| 黑麦草青贮 Ryegrass silage | 75.43±0.09c | 23.27±6.48ab | 14.25±0.33e | 9.80±0.27de | 67.12±0.18b | 17.84±0.32d |
| 葵花头 Sunflower head | 77.76±0.31bc | 13.42±1.20e | 16.76±3.41d | 12.50±0.15bc | 73.46±1.17a | 13.12±0.03g |
| 葵花头青贮 Sunflower head silage | 77.23±0.35bc | 22.38±1.44abc | 18.36±0.31cd | 11.77±0.36c | 56.54±1.36de | 21.09±0.06b |
| 芦苇草 Alfa | 68.67±3.05d | 9.93±1.34f | 19.02±0.91bcd | 7.21±0.08f | 66.33±1.34bc | 23.74±0.01a |
| 芦苇草青贮 Alfa silage | 63.56±0.06e | 16.31±1.38cde | 15.87±0.95de | 9.74±0.33de | 65.66±0.81bc | 18.04±0.57d |
| 3年生柠条 Three-year caragana | 83.31±0.14a | 28.56±5.11a | 27.63±0.81a | 16.79±0.21a | 54.46±5.27e | 16.99±0.14e |
| 3年生柠条青贮 Three-year caragana silage | 83.73±1.35a | 28.56±5.11a | 28.92±0.96a | 16.75±0.17a | 59.72±0.55cde | 20.46±0.02c |
| 燕麦草 Oat grass | 74.69±0.19c | 21.81±0.10bcd | 20.60±0.06bc | 10.22±0.42d | 64.18±0.12bc | 14.02±0.03f |
| 燕麦草青贮 Oat grass silage | 71.48±0.04d | 23.17±1.97ab | 21.71±1.29b | 12.46±0.11bc | 56.72±1.84de | 20.11±0.13c |
2.3 不同粗饲料对滩羊瘤胃菌群的影响
2.3.1 操作分类单元(OTU)聚类分析
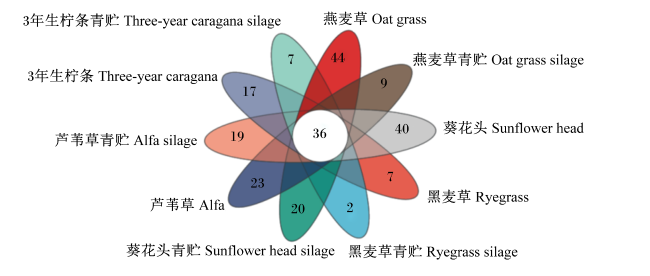
2.3.2 α多样性分析
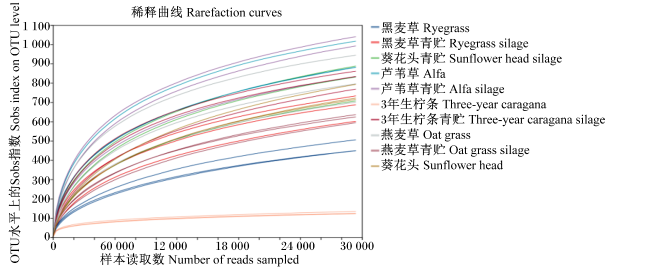
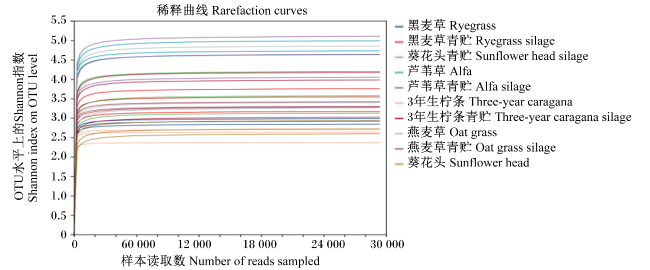
表4 不同粗饲料对滩羊瘤胃菌群α多样性的影响Table 4 Effects of different roughages on α diversity of rumen microbiota of Tan sheep |
| 项目 Items | Sobs指数 Sobs index | Shannon指数 Shannon index | Simpson指数 Simpson index | Ace指数 Ace index | Chao1指数 Chao1 index | 覆盖度 Coverage | |
|---|---|---|---|---|---|---|---|
| 黑麦草 Ryegrass | 467.67±32.33f | 2.91±0.07d | 0.15±0.02b | 722.38±84.84f | 673.81±50.30e | 0.99±0.00 | |
| 黑麦草青贮 Ryegrass silage | 673.67±67.00de | 3.49±0.30cd | 0.10±0.01bcd | 909.36±61.15de | 918.51±68.68cd | 0.99±0.00 | |
| 葵花头 Sunflower head | 743.33±43.15cd | 2.35±0.17f | 0.28±0.05a | 1 013.30±62.73cd | 1 012.54±72.94bc | 0.99±0.00 | |
| 葵花头青贮 Sunflower head silage | 808.67±92.54bc | 3.63±0.54c | 0.11±0.04bc | 1 063.37±101.25bc | 1 079.29±97.21ab | 0.99±0.00 | |
| 芦苇草 Alfa | 926.67±78.23ab | 4.78±0.18a | 0.02±0.00d | 1 186.17±45.65a | 1 179.88±57.30a | 0.99±0.00 | |
| 芦苇草青贮 Alfa silage | 955.00±108.35a | 4.30±0.08b | 0.04±0.03cd | 1 194.84±115.74a | 1 203.63±105.39a | 0.99±0.00 | |
| 3年生柠条 Three-year caragana | 126.67±6.43g | 2.57±0.18e | 0.14±0.05b | 180.79±22.26g | 168.04±9.17f | 1.00±0.00 | |
| 3年生柠条青贮 Three-year caragana silage | 821.00±47.84bc | 3.72±0.62c | 0.12±0.07bc | 1 059.17±9.58bc | 1 097.23±35.34ab | 0.99±0.00 | |
| 燕麦草 Oat grass | 813.33±122.92bc | 3.84±0.88c | 0.11±0.08bc | 1 016.70±108.59cd | 1 018.92±104.76bc | 0.99±0.00 | |
| 燕麦草青贮 Oat grass silage | 618.00±21.63e | 3.33±0.08cd | 0.10±0.02bcd | 859.00±13.18e | 855.80±30.08d | 0.99±0.00 | |
2.3.3 β多样性分析
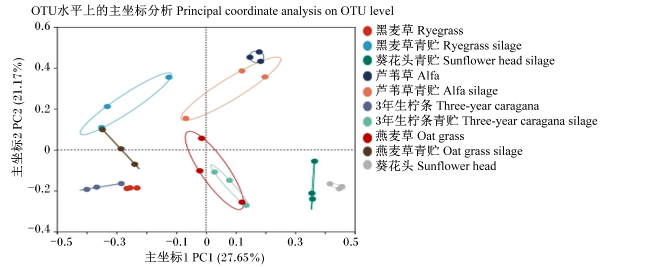
2.3.4 菌群组成分析
2.3.4.1 在门水平上组成
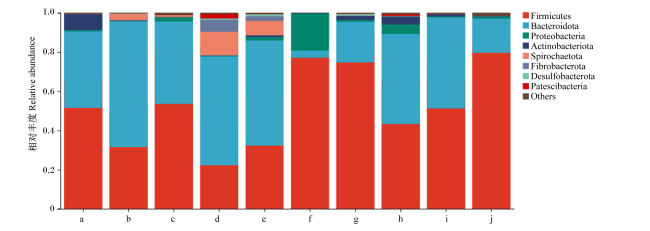
图5 滩羊瘤胃菌群在门水平上组成a:黑麦草 ryegrass;b:黑麦草青贮 ryegrass silage;c:葵花头青贮 sunflower head silage;d:芦苇草 alfa;e:芦苇草青贮 alfa silage;f:3年生柠条 three-year caragana;g:3年生柠条青贮 three-year caragana silage;h:燕麦草 oat grass;i:燕麦草青贮 oat grass silage;j:葵花头 sunflower head。图6同 the same as Fig.6。 Firmicutes:厚壁菌门;Bacteroidota:拟杆菌门;Proteobacteria:变形菌门;Actinobacteriota:放线菌门;Spirochaetota:螺旋体门;Fibrobacterota:纤维杆菌门;Desulfobacterota:脱硫杆菌门;Patescibacteria:髌骨菌门;Others:其他。 Fig.5 Composition of rumen microbiota of Tan sheep at phylum level |
表5 不同粗饲料对滩羊瘤胃菌群在门水平上相对丰度的影响Table 5 Effects of different roughages on relative abundance of rumen microbiota of Tan sheep at phylum level |
| 项目 Items | 黑麦草 Ryegrass | 黑麦草青贮 Ryegrass silage | 葵花头青贮 Sunflower head silage | 芦苇草 Alfa | 芦苇草青贮 Alfa silage | 3年生柠条 Three-year caragana | 3年生 柠条青贮 Three-year caragana silage | 燕麦草 Oat grass | 燕麦草青贮 Oat grass silage | 葵花头 Sunflower head |
|---|---|---|---|---|---|---|---|---|---|---|
| 厚壁菌门 Firmicutes | 0.61±0.08bcd | 0.44±0.11cde | 0.71±0.16ab | 0.30±0.12e | 0.43±0.14de | 0.78±0.01ab | 0.80±0.08ab | 0.62±0.18abcd | 0.63±0.11abc | 0.81±0.03a |
| 拟杆菌门 Bacteroidota | 0.30±0.09bc | 0.52±0.10a | 0.25±0.15cd | 0.51±0.13a | 0.46±0.14ab | 0.06±0.12d | 0.16±0.07cd | 0.29±0.20bc | 0.35±0.11abc | 0.15±0.04cd |
| 变形菌门 Proteobacteria | 0.01±0.00b | 0.01±0.01b | 0.02±0.00b | 0.00±0.00b | 0.03±0.03b | 0.17±0.13a | 0.01±0.00b | 0.03±0.03b | 0.00±0.00b | 0.01±0.00b |
| 放线菌门 Actinobacteriota | 0.08±0.00a | 0.01±0.01c | 0.00±0.00c | 0.01±0.01c | 0.01±0.00c | 0.00±0.00c | 0.01±0.01c | 0.04±0.01b | 0.01±0.00c | 0.00±0.00c |
| 螺旋体门 Spirochaetota | 0.00±0.00c | 0.01±0.02c | 0.00±0.00c | 0.10±0.01a | 0.04±0.03b | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c |
| 纤维杆菌门 Fibrobacterota | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.05±0.03a | 0.02±0.01b | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c |
| 脱硫杆菌门 Desulfobacterota | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.01±0.00a | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b |
| 髌骨菌门 Patescibacteria | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b |
| 其他 Others | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.01±0.00a |
2.3.4.2 在属水平上组成
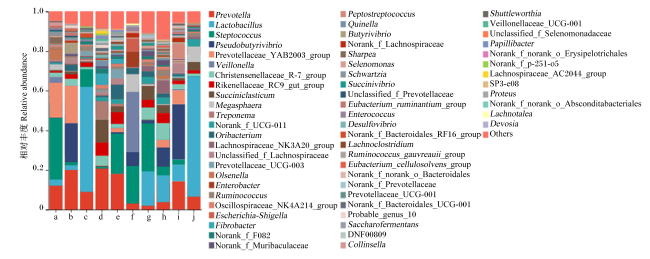
图6 滩羊瘤胃菌群在属水平上组成Prevotella:普雷沃氏菌属;Lactobacillus:乳杆菌属;Steptococcus:链球菌属;Pseudobutyrivibrio:假丁酸弧菌属;Prevotellaceae_YAB2003_group:普雷沃氏菌科YAB2003群;Veillonella:韦荣氏球菌属;Christensenellaceae_R-7_group:克里斯滕森菌科R-7群;Rikenellaceae_RC9_gut_group:理研菌科RC9肠道群;Succiniclasticum:琥珀酸菌属;Megasphaera:巨球型菌属;Treponema:密螺旋体属;Norank_f_UCG-011:未定级UCG-011;Lachnospiraceae_NK3A20_group:毛螺菌科NK3A20群;Unclassified_f_Lachnospiraceae:未分类毛螺菌科;Prevotellaceae_UCG-003:普雷沃氏菌科UCG-003;Olsenella:欧陆森氏菌属;Enterobacter:肠杆菌属;Ruminococcus:瘤胃球菌属;Oscillospiraceae_NK4A214_group:颤螺菌科NK4A214群;Escherichia-Shigella:埃希氏菌-志贺氏菌属; Fibrobacter:纤维杆菌属;Norank_f_F082:未定级F082;Norank_f_Muribaculaceae:未定级鼠杆菌科;Peptostreptococcus:消化链球菌属;Quinella:奎因氏菌属;Butyrivibrio:丁酸弧菌属;Norank_f_Lachnospiraceae:未定级毛螺菌科;Sharpea:夏普氏菌属;Selenomonas:月形单胞菌属;Schwartzia:施氏菌属;Succinivibrio:琥珀酸弧菌属;Unclassified_f_Prevotellaceae:未分类普雷沃氏菌科;Enterococcus:肠球菌属;Desulfovibrio:脱硫弧菌属;Norank_f_Bacteroidales_RF16_group:未定级拟杆菌目RF16群;Norank_f_norank_o_Bacteroidales:未定级拟杆菌目;Norank_f_Prevotellaceae:未定级普雷沃氏菌科;Prevotellaceae_UCG-001:普雷沃氏菌科UCG-001;Norank_f_Bacteroidales_UCG-001:未定级拟杆菌目UCG-001;Saccharofermentans:糖发酵菌属;Collinsella:柯林斯氏菌属;Shuttleworthia:萨特沃氏菌属;Veillonellaceae_UCG-001:韦荣氏球菌科UCG-001;Unclassified_f_Selenomonadaceae:未分类月形单胞菌科;Papillibacter:乳头杆菌属;Norank_f_norank_o_Erysipelotrichales:未定级丹毒丝菌目;Lachnospiraceae_AC2044_group:毛螺菌科AC2044群;Proteus:变形杆菌属;Lachnotalea:毛杆菌属;Devosia:德沃斯氏菌属;Others:其他。 Fig.6 Composition of rumen microbiota of Tan sheep at genus level |
表6 不同粗饲料对滩羊瘤胃菌群在属水平上相对丰度的影响Table 6 Effects of different roughages on relative abundance of rumen microbiota of Tan sheep at genus level |
| 项目 Items | 黑麦草 Ryegrass | 黑麦草青贮 Ryegrass silage | 葵花头青贮 Sunflower head silage | 芦苇草 Alfa | 芦苇草青贮 Alfa silage | 3年生柠条 Three-year caragana | 3年生 柠条青贮 Three-year caragana silage | 燕麦草 Oat grass | 燕麦草青贮 Oat grass silage | 葵花头 Sunflower head | |
|---|---|---|---|---|---|---|---|---|---|---|---|
| 普雷沃氏菌属 Prevotella | 0.14±0.02cd | 0.30±0.13bc | 0.16±0.11bcd | 0.36±0.13a | 0.30±0.11ab | 0.05±0.02d | 0.07±0.05cd | 0.17±0.15bcd | 0.18±0.04bcd | 0.10±0.03cd | |
| 乳杆菌属 Lactobacillus | 0.05±0.01de | 0.01±0.01e | 0.48±0.13b | 0.00±0.00e | 0.03±0.04de | 0.00±0.00e | 0.19±0.08c | 0.13±0.08cd | 0.08±0.05de | 0.64±0.07a | |
| 链球菌属 Steptococcus | 0.33±0.07a | 0.01±0.01d | 0.10±0.02cd | 0.01±0.00d | 0.08±0.12cd | 0.20±0.03bc | 0.29±0.08ab | 0.18±0.17bc | 0.04±0.01d | 0.00±0.00d | |
| 假丁酸弧菌属 Pseudobutyrivibrio | 0.01±0.00c | 0.17±0.06ab | 0.00±0.00c | 0.00±0.00c | 0.02±0.02c | 0.13±0.06b | 0.01±0.01c | 0.02±0.02c | 0.22±0.05a | 0.00±0.00c | |
| 普雷沃氏菌科YAB2003群 Prevotellaceae_YAB2003_group | 0.14±0.07ab | 0.17±0.05a | 0.00±0.00c | 0.01±0.01c | 0.01±0.01c | 0.00±0.00c | 0.00±0.00c | 0.06±0.06bc | 0.14±0.11ab | 0.00±0.00c | |
| 韦荣氏球菌属 Veillonella | 0.03±0.01b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.25±0.13a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 克里斯滕森菌科R-7群 Christensenellaceae_R-7_group | 0.02±0.01bc | 0.02±0.01bc | 0.01±0.00c | 0.04±0.01ab | 0.02±0.00bc | 0.00±0.00c | 0.05±0.01a | 0.05±0.03a | 0.02±0.01bc | 0.01±0.00c | |
| 理研菌科RC9肠道群 Rikenellaceae_RC9_gut_group | 0.01±0.00cd | 0.02±0.01bc | 0.02±0.00bc | 0.05±0.02a | 0.05±0.01a | 0.00±0.00d | 0.03±0.01b | 0.03±0.01b | 0.02±0.01bc | 0.02±0.00bc | |
| 琥珀酸菌属 Succiniclasticum | 0.01±0.00bc | 0.03±0.02abc | 0.01±0.00bc | 0.06±0.05a | 0.03±0.02abc | 0.00±0.00c | 0.04±0.03ab | 0.03±0.01abc | 0.02±0.02bc | 0.02±0.02bc | |
| 巨球型菌属 Megasphaera | 0.02±0.01ab | 0.02±0.03ab | 0.02±0.01ab | 0.00±0.00b | 0.00±0.00b | 0.07±0.07a | 0.01±0.00b | 0.00±0.00b | 0.03±0.05ab | 0.04±0.05ab | |
| 密螺旋体属 Treponema | 0.00±0.00c | 0.01±0.02c | 0.00±0.00c | 0.10±0.01a | 0.04±0.03b | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | |
| 未定级UCG-011 Norank_f_UCG-011 | 0.00±0.00c | 0.01±0.01bc | 0.01±0.00bc | 0.02±0.00ab | 0.03±0.01a | 0.00±0.00c | 0.03±0.01a | 0.02±0.01ab | 0.01±0.00bc | 0.03±0.00a | |
| Oribacterium | 0.00±0.00c | 0.02±0.01abc | 0.00±0.00c | 0.01±0.01bc | 0.04±0.03a | 0.03±0.01ab | 0.02±0.01abc | 0.01±0.01bc | 0.01±0.00bc | 0.00±0.00c | |
| 毛螺菌科NK3A20群 Lachnospiraceae_NK3A20_group | 0.01±0.00bc | 0.00±0.00c | 0.01±0.00bc | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.02±0.01b | 0.04±0.02a | 0.01±0.00bc | 0.01±0.00bc | |
| 未分类毛螺菌科 Unclassified_f_Lachnospiraceae | 0.01±0.00bc | 0.02±0.01ab | 0.00±0.00c | 0.01±0.00bc | 0.02±0.01ab | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.03±0.02a | 0.00±0.00c | |
| 普雷沃氏菌科UCG-003 Prevotellaceae_UCG-003 | 0.00±0.00c | 0.00±0.00c | 0.01±0.01bc | 0.02±0.01b | 0.06±0.03a | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | |
| 欧陆森氏菌属 Olsenella | 0.06±0.01a | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.01±0.01b | 0.00±0.00c | 0.00±0.00c | |
| 肠杆菌属 Enterobacter | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.08±0.02a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 瘤胃球菌属 Ruminococcus | 0.00±0.00c | 0.00±0.00c | 0.02±0.01a | 0.01±0.00b | 0.01±0.00b | 0.00±0.00c | 0.01±0.00b | 0.02±0.01a | 0.01±0.00b | 0.01±0.00b | |
| 颤螺菌科NK4A214群 Oscillospiraceae_ NK4A214_group | 0.00±0.00c | 0.00±0.00c | 0.01±0.00b | 0.01±0.00b | 0.01±0.00b | 0.00±0.00c | 0.01±0.00b | 0.02±0.01a | 0.00±0.00c | 0.01±0.00b | |
| 埃希氏菌-志贺氏菌属 Escherichia-Shigella | 0.00±0.00c | 0.00±0.01c | 0.00±0.00c | 0.00±0.00c | 0.02±0.03b | 0.06±0.01a | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | |
| 纤维杆菌属 Fibrobacter | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.05±0.03a | 0.02±0.01b | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | |
| 未定级F082 Norank_f_F082 | 0.00±0.00c | 0.00±0.00c | 0.01±0.00b | 0.02±0.01a | 0.01±0.00b | 0.00±0.00c | 0.01±0.00b | 0.01±0.00b | 0.00±0.00c | 0.01±0.00b | |
| 未定级鼠杆菌科 Norank_f_Muribaculaceae | 0.00±0.00c | 0.01±0.00b | 0.00±0.00c | 0.01±0.01b | 0.00±0.00c | 0.00±0.00c | 0.02±0.00a | 0.01±0.01b | 0.00±0.00c | 0.00±0.00c | |
| 消化链球菌属 Peptostreptococcus | 0.01±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00b | 0.00±0.00b | 0.00±0.00b | 0.04±0.03a | 0.00±0.00b | |
| 奎因氏菌属 Quinella | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.01±0.01a | 0.01±0.01a | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 丁酸弧菌属 Butyrivibrio | 0.00±0.00b | 0.02±0.03a | 0.00±0.00b | 0.00±0.00b | 0.01±0.01ab | 0.00±0.00b | 0.00±0.00b | 0.01±0.00ab | 0.01±0.00ab | 0.00±0.00b | |
| 未定级毛螺菌科 Norank_f_Lachnospiraceae | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.01±0.01a | 0.00±0.00b | 0.00±0.00b | 0.01±0.01a | 0.00±0.00b | |
| 夏普氏菌属 Sharpea | 0.04±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 月形单胞菌属 Selenomonas | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.01±0.00a | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 施氏菌属 Schwartzia | 0.02±0.00a | 0.02±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 琥珀酸弧菌属 Succinivibrio | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 未分类普雷沃氏菌科 Unclassified_f_Prevotellaceae | 0.01±0.00a | 0.01±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.01±0.00a | |
| Eubacterium_ ruminantium_group | 0.00±0.00c | 0.01±0.00b | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.02±0.01a | 0.00±0.00c | |
| 肠球菌属 Enterococcus | 0.01±0.00b | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.00±0.00c | 0.02±0.00a | 0.00±0.00c | 0.00±0.00c | 0.01±0.00b | 0.00±0.00c | |
| 脱硫弧菌属 Desulfovibrio | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.01±0.00a | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 未定级拟杆菌目RF16群 Norank_f_Bacteroidales_ RF16_group | 0.00±0.00b | 0.00±0.00b | 0.02±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| Lachnoclostridium | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| Ruminococcus_gauvreauii_group | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| Eubacterium_cellulosolvens_ group | 0.01±0.00a | 0.01±0.00a | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.01b | 0.00±0.00b | 0.00±0.00b | |
| 未定级拟杆菌目 Norank_f_norank_o_Bacteroidales | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 未定级普雷沃氏菌科 Norank_f_Prevotellaceae | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 普雷沃氏菌科UCG-001 | 0.00±0.00b | 0.00±0.00b | 0.01±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| Prevotellaceae_UCG-001 | |||||||||||
| 未定级拟杆菌目UCG-001 Norank_f_Bacteroidales_ UCG-001 | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| Probable_genus_10 | 0.00±0.00b | 0.01±0.01a | 0.00±0.00b | 0.01±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 糖发酵菌属 Saccharofermentans | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| DNF00809 | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | |
| 柯林斯氏菌属 Collinsella | 0.01±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 萨特沃氏菌属 Shuttleworthia | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | |
| 韦荣氏球菌科UCG001 Veillonellaceae_UCG-001 | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 未分类月形单胞菌科 Unclassified_f_Selenomonadaceae | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | |
| 乳头杆菌属 Papillibacter | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.01a | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 未定级丹毒丝菌目 Norank_f_norank_o_ Erysipelotrichales | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| Norank_f_p-251-o5 | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | |
| 毛螺菌科AC2044群 Lachnospiraceae_AC2044_group | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| SP3-e08 | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 变形杆菌属 Proteus | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| Norank_f_norank_o_ Absconditabacteriales | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.01a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 毛杆菌属 Lachnotalea | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | |
| 德沃斯氏菌属 Devosia | 0.00±0.00b | 0.01±0.00a | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.00±0.00b | 0.01±0.00a | |
| 其他 Others | 0.04±0.01d | 0.05±0.01cd | 0.06±0.01cd | 0.06±0.02cd | 0.07±0.01bc | 0.05±0.01cd | 0.09±0.02ab | 0.11±0.04a | 0.05±0.00cd | 0.04±0.01d | |
2.3.5 瘤胃菌群功能预测
表7 滩羊瘤胃菌群KEGG通路分析Table 7 KEGG pathway analysis of rumen microbiota of Tan sheep |
| 一级通路 Primary pathway | 二级通路 Secondary pathway | 黑麦草 Ryegrass | 黑麦草青贮 Ryegrass silage | 葵花头青贮 Sunflower head silage | 芦苇草 Alfa | 芦苇 草青贮 Alfa silage | 3年生柠条 Three-year caragana | 3年生 柠条青贮 Three-year caragana silage | 燕麦草 Oat grass | 燕麦草青贮 Oat grass silage | 葵花头 Sunflower head |
|---|---|---|---|---|---|---|---|---|---|---|---|
| 新陈代谢 Metabolism | 全局和概述图谱 Global and overview maps | 21 538 989.05 ±401 625.48de | 23 852 938.70 ±1 392 001.44abc | 17 071 593.47 ±1 994 068.95f | 24 397 442.84 ±342 439.04ab | 24 832 881.36 ±835 215.68a | 23 329 065.38 ±224 551.4abcd | 20 807 666.78 ±869 892.88e | 22 116 748.62 ±1 498 678.54cde | 22 775 490.57 ±1 347 216.84bcd | 13 337 194.91 ±1 215 069.78g |
| 碳水化合物代谢 Carbohydrate metabolism | 5 457 514.17 ±88 376.53cd | 6 015 613.26 ±507 558.25ab | 4 351 426.98 ±483 274.94e | 5 807 012.28 ±210 349.76abc | 6 165 897.86 ±282 148.51a | 5 524 887.06 ±248 655.89bcd | 5 046 344.74 ±108 820.04d | 5 359 618.14 ±304 297.33cd | 5 667 624.28 ±439 380.41abc | 3 297 885.02 ±210 305.52f | |
| 氨基酸代谢 Amino acid metabolism | 3 652 171.91 ±89 462.92abc | 4 020 490.96 ±274 216.53a | 2 934 601.25 ±364 007.29cd | 4 304 009.43 ±76 218.24a | 4 319 304.67 ±141 166.07a | 3 979 303.38 ±11 906.61a | 3 632 068.31 ±174 754.13abc | 3 843 181.52 ±389 859.10ab | 3 794 624.11 ±199 301.47bc | 2 339 431.55 ±229 686.49d | |
| 辅助因子和维 生素代谢 Metabolism of cofactors and vitamins | 2 209 440.52 ±43 671.71c | 2 620 644.47 ±114 678.22a | 1 702 085.07 ±271 426.46d | 2 671 847.81 ±33 645.39a | 2 672 618.61 ±142 296.43a | 2 701 939.04 ±93 877.39a | 2 142 383.29 ±156 158.22c | 2 339 349.63 ±159 151.84bc | 2 481 116.01 ±113 541.74ab | 1 336 128.87 ±196 417.12e | |
| 能量代谢 Energy metabolism | 2 109 396.10 ±51 968.74de | 2 551 133.75 ±102 895.66a | 1 689 053.99 ±238 916.41f | 2 521 409.79 ±37 488.30ab | 2 531 887.92 ±93 965.66ab | 2 306 047.87 ±17 797.25bcd | 1 973 243.51 ±132 912.45e | 2 249 087.91 ±171 396.48cd | 2 430 742.45 ±196 816.97abc | 1 300 309.77 ±107 654.16g | |
| 核苷酸代谢 Nucleotide metabolism | 1 632 040.98 ±15 438.54cd | 1 750 307.20 ±115 017.70abc | 1 375 108.12 ±122 962.76e | 1 791 474.61 ±59 827.70ab | 1 811 427.90 ±43 778.52a | 1 631 263.04 ±10 671.70cd | 1 535 047.15 ±30 063.06d | 1 633 314.80 ±49 196.56cd | 1 665 059.66 ±114 561.89cd | 1 072 066.84 ±68 793.49f | |
| 聚糖的生物 合成和代谢 Glycan biosynthesis and metabolism | 928 089.23 ±72 339.76b | 1 144 039.73 ±136 844.98a | 756 344.99 ±169 684.05bc | 1 188 505.56 ±93 953.60a | 1 152 332.97 ±132 522.86a | 917 924.81 ±54 035.92b | 770 987.90 ±65 634.79b | 919 304.11 ±146 652.86b | 939 158.25 ±117 369.24b | 567 077.62 ±82 836.76c | |
遗传信息处理 Genetic information processing | 翻译 Translation | 2 126 531.57 ±20 084.84abc | 2 117 840.17 ±101 907.66bc | 1 683 908.29 ±131 332.24d | 2 261 541.77 ±35 075.94a | 2 238 591.89 ±27 213.33ab | 1 999 891.17 ±14 406.67c | 2 013 827.7 ±54 843.00c | 2 081 768.41 ±97 268.95c | 2 044 539.68 ±116 968.81c | 1 310 509.11 ±107 581.17e |
| 复制和修复 Replication and repair | 1 797 663.95 ±18 783.73bc | 1 857 403.13 ±95 755.71ab | 1 449 680.54 ±123 580.35d | 1 965 926.10 ±26 913.98a | 1 937 124.56 ±33 658.70a | 1 713 129.62 ±16 460.01c | 1 684 523.68 ±52 369.11c | 1 781 237.83 ±85 370.79bc | 1 772 860.39 ±108 261.95bc | 1 123 602.47 ±87 807.53e | |
| 环境信息处理 Environmental information processing | 膜运输 Membrane transport | 1 979 893.10 ±199 031.18b | 1 686 674.64 ±197 615.83bcd | 1 306 671.91 ±94 720.10de | 1 461 447.11 ±128 041.65cd | 1 662 343.87 ±374 632.04bcd | 2 572 212.93 ±112 802.03a | 1 867 275.98 ±85 257.91b | 1 770 380.13 ±409 273.67bc | 1 965 323.21 ±257 077.55b | 942 065.44 ±76 765.13e |
 京公网安备 11010802041926号


