研究论文

壳寡糖缓解热应激肉鸡肠道屏障损伤的作用研究

  • 王振锋 ,
  • 张迦 ,
  • 高金稔 ,
  • 兰瑞霞 , **
展开
  • 广东海洋大学滨海农业学院, 湛江 524088
**兰瑞霞,讲师,硕士生导师,E-mail:

*同等贡献作者

王振锋(2003—),男,广东茂名人,本科生,研究方向为动物营养与饲料科学。E-mail:

Office editor: 田艳明

收稿日期: 2025-09-25

  网络出版日期: 2026-04-14

基金资助

广东海洋大学科研启动项目(R18005)

广东海洋大学滨海农业学院大学生创新项目

Effects of Chitosan Oligosaccharide on Alleviating Intestinal Barrier Damage in Heat-Stressed Broilers

  • WANG Zhenfeng ,
  • ZHANG Jia ,
  • GAO Jinren ,
  • LAN Ruixia , **
Expand
  • College of Coastal Agriculture Sciences, Guangdong Ocean University, Zhanjiang 524088, China
**lecturer, E-mail:

*Contributed equally

Received date: 2025-09-25

  Online published: 2026-04-14

摘要

本试验旨在探究壳寡糖(COS)对热应激肉鸡肠道屏障损伤的缓解作用。选取28日龄体重相近的雄性爱拔益加(AA)肉鸡144只,随机分为3组,每组6个重复,每个重复8只鸡。对照组(CON组)肉鸡饲养在温度为(24±1) ℃的鸡舍;热应激组(HS组)和热应激COS组(HSC-200组)肉鸡饲养在08:00—18:00温度为(34±1) ℃,其余时间温度为(24±1) ℃的鸡舍。同时,CON组和HS组饲喂基础饲粮,HSC-200组饲喂在基础饲粮的基础上添加200 mg/kg COS的饲粮。试验期14 d。结果表明:1)与CON组相比,HS组血清D-乳酸(D-LA)含量显著提高(P<0.05),空肠闭合蛋白(Occludin)mRNA相对表达量显著降低(P<0.05);与HS组相比,HSC-200组血清D-LA含量显著降低(P<0.05),空肠Occludin mRNA相对表达量显著提高(P<0.05)。2)与CON组相比,HS组空肠Toll样受体4(TLR4)、核因子-κB p65亚基(NF-κB p65)、白细胞介素-6(IL-6)、NOD样受体热蛋白结构域相关蛋白3(NLRP3)、半胱天冬酶(Caspase)1和白细胞介素-18(IL-18)mRNA相对表达量显著提高(P<0.05);与HS组相比,HSC-200组空肠TLR4、IL-6、NLRP3、Caspase 1和IL-18 mRNA相对表达量显著降低(P<0.05)。3)与CON组相比,HS组空肠上皮细胞凋亡率以及热休克蛋白(Hsp)70、Hsp90、Caspase 3和B细胞淋巴瘤-2相关X蛋白(Bax)mRNA相对表达量显著提高(P<0.05),空肠B细胞淋巴瘤-2(Bcl-2)mRNA相对表达量和Bcl-2/Bax值显著降低(P<0.05);与HS组相比,HSC-200组空肠上皮细胞凋亡率以及Hsp70、Hsp90、Caspase 3和Bax mRNA相对表达量显著降低(P<0.05),空肠Bcl-2 mRNA相对表达量和Bcl-2/Bax值显著提高(P<0.05)。4)与CON组相比,HS组空肠线粒体融合蛋白(MFN)1、MFN2和视神经萎缩蛋白1(OPA1)mRNA相对表达量显著降低(P<0.05),空肠线粒体裂变因子(MFF)、E3泛素连接酶(Parkin)和微管相关蛋白1轻链3Ⅱ(LC3Ⅱ)mRNA相对表达量显著提高(P<0.05);与HS组相比,HSC-200组空肠MFN1和OPA1 mRNA相对表达量显著提高(P<0.05),空肠ParkinLC3 mRNA相对表达量显著降低(P<0.05)。综上所述,COS通过改善热应激肉鸡肠上皮细胞线粒体功能,进而缓解炎症反应,减少细胞凋亡,最终发挥保护肠道屏障的作用。

本文引用格式

王振锋 , 张迦 , 高金稔 , 兰瑞霞 . 壳寡糖缓解热应激肉鸡肠道屏障损伤的作用研究[J]. 动物营养学报, 2026 , 38(4) : 2611 -2622 . DOI: 10.12418/CJAN2026.210

Abstract

The aim of this study was to investigate the effects of chitosan oligosaccharide (COS) on alleviating intestinal barrier damage in heat-stressed broilers. A total of 144 male Arbor Acres (AA) broilers of 28-day-old with similar body weight were randomly divided into three groups, with six replicates in each group and eight broilers in each replicate. The broilers in the control group (CON group) were housed in a temperature-controlled room of (24±1) ℃. The broilers in the heat stress group (HS group) and the heat stress with COS supplementation group (HSC-200 group) were housed in a temperature-controlled room of (34±1) ℃ from 08:00 to 18:00, and the rest time was (24±1) ℃. The CON and HS groups were fed a basal diet, and the HSC-200 group was fed the basal diet supplemented with 200 mg/kg COS. The experiment lasted for 14 days. The results showed as follows: 1) compared with the CON group, the serum D-lactate (D-LA) content in the HS group was significantly increased (P<0.05), and the jejunal Occludin mRNA relative expression level was significantly down-regulated (P<0.05). Compared with the HS group, the serum D-LA content in the HSC-200 group was significantly decreased (P<0.05), and the jejunal Occludin mRNA relative expression level was significantly up-regulated (P<0.05). 2) Compared with the CON group, the jejunal mRNA relative expression levels of Toll-like receptor 4 (TLR4), nuclear factor-kappa B p65 subunit (NF-κB p65), interleukin-6 (IL-6), NOD-like receptor thermal protein domain associated protein 3 (NLRP3), Caspase 1 and interleukin-18 (IL-18) in the HS group were significantly up-regulated (P<0.05). Compared with the HS group, the jejunal mRNA relative expression levels of TLR4, IL-6, NLRP3, Caspase 1 and IL-18 in the HSC-200 group were significantly down-regulated (P<0.05). 3) Compared with the CON group, the apoptosis rate of jejunal epithelial cells in the HS group was significantly increased (P<0.05), the jejunal mRNA relative expression levels of heat shock protein (Hsp) 70, Hsp90, Caspase 3 and B-cell lymphoma-2-associated X protein (Bax) were significantly up-regulated (P<0.05), and the jejunal mRNA relative expression levels of B-cell lymphoma-2 (Bcl-2) and the ratio of Bcl-2 to Bax were significantly down-regulated (P<0.05). Compared with the HS group, the apoptosis rate of jejunal epithelial cells in the HSC-200 group was significantly decreased (P<0.05), the jejunal mRNA relative expression levels of Hsp70, Hsp90, Caspase 3 and Bax were significantly down-regulated (P<0.05), and the jejunal mRNA relative expression levels of Bcl-2 and the ratio of Bcl-2 to Bax were significantly up-regulated (P<0.05). 4) Compared with the CON group, the jejunal mRNA relative expression levels of mitofusin (MFN) 1, MFN2 and optic atrophy 1 (OPA1) in the HS group were significantly down-regulated (P<0.05), while the jejunal mRNA relative expression levels of mitochondrial fission factor (MFF), E3 ubiquitin ligase (Parkin) and microtubule-associated protein 1 light chain 3Ⅱ (LC3Ⅱ) were significantly up-regulated (P<0.05). Compared with the HS group, the jejunal mRNA relative expression levels of MFN1 and OPA1 in the HSC-200 group were significantly up-regulated (P<0.05), while the jejunal mRNA relative expression levels of Parkin and LC3Ⅱ were significantly down-regulated (P<0.05). In conclusion, COS can maintain the mitochondrial function of intestinal epithelial cells in heat-stressed broilers, followed by alleviating inflammatory response, decreasing apoptosis, and finally protecting the intestinal barrier function.

热应激是畜牧业夏季生产过程中的关键共性问题。肉鸡因体温高、基础代谢旺盛、全身覆盖羽毛且缺乏汗腺,极易受热应激影响[1]。热应激会降低肉鸡生长性能,导致内分泌紊乱、组织器官氧化损伤及炎症反应,甚至导致肉鸡死亡[2]。肠道是热应激的靶器官,热应激导致肠道缺血、缺氧,诱发肠道氧化损伤和炎症反应,使肉鸡小肠形态结构发生改变,消化酶活性降低,营养物质转运能力下降,肠上皮细胞凋亡加剧,肠道屏障出现损伤,最终导致生长性能和养殖效益下降[3-4]。因此,改善热应激肉鸡的肠道健康水平,是肉鸡夏季生产提质增效的关键。热应激导致的肠道屏障损伤与肠道通透性增加、氧化损伤、炎症反应、细胞过度凋亡和线粒体功能障碍相关[5-6]。线粒体是细胞的“能量工厂”,维持线粒体正常功能对细胞能量代谢和细胞生存调控具有重要意义[7]。线粒体功能的稳定主要与线粒体生物发生、融合和分裂及线粒体自噬的动态平衡相关[8-9]。线粒体功能异常可能引发异常线粒体积累、线粒体膜电位下降、ATP合成受阻以及活性氧(ROS)过量产生等级联反应,激活Toll样受体4(TLR4)/核因子-κB(NF-κB)和NOD样受体热蛋白结构域相关蛋白3(NLRP3)炎症通路,促进促炎因子的分泌导致细胞凋亡,最终导致肠道屏障损伤[6,10]。相关研究也已证实,热应激引起的肉鸡肠道氧化损伤和炎症反应在肠上皮细胞凋亡和屏障损伤中有重要影响[4-5]。不过,关于热应激对肠上皮细胞线粒体功能的影响及线粒体功能损伤对肠道屏障损伤影响的研究较少。
壳寡糖(chitosan oligosaccharide,COS)是由2~20个氨基葡萄糖通过β-1,4-糖苷键连接而成的碱性氨基寡糖,具有抗炎、抗氧化和抗凋亡等多种生物学功能[11]。本课题组前期研究表明,COS能通过修复热应激肉鸡小肠形态结构,提高小肠消化吸收能力及抗氧化能力,改善生长性能[3]。同时,COS能通过改善热应激肉鸡小肠抗氧化能力和炎性反应缓解肠道屏障损伤[12]。但是,COS是否能通过维持热应激肉鸡肠上皮细胞线粒体功能缓解炎性损伤和细胞凋亡,进而最终缓解肠道屏障损伤还未见相关报道。因此,本研究旨在探究COS对热应激肉鸡肠道屏障、炎症反应、肠上皮细胞凋亡和线粒体功能的影响,以期为将COS应用于缓解热应激肉鸡肠道屏障损伤提供参考。

1 材料与方法

1.1 试验动物和试验设计

选取28日龄体重相近的雄性爱拔益加(AA)肉鸡144只,随机分为3组,每组6个重复,每个重复8只鸡。对照组(CON组)肉鸡饲养在温度为(24±1) ℃的鸡舍;热应激组(HS组)和热应激COS组(HSC-200组)饲养在08:00—18:00温度为(34±1) ℃,其余时间温度为(24±1) ℃的鸡舍。同时,CON组和HS组饲喂基础饲粮,HSC-200组饲喂在基础饲粮的基础上添加200 mg/kg COS的饲粮。试验期14 d。COS添加量和基础饲粮组成及营养水平见课题组前期报道[3]。COS纯度为93.6%,平均分子质量为1 768 u,脱乙酰度≥90%。
试验期间肉鸡自由采食和饮水,按饲养管理和免疫程序进行管理和免疫接种。肉鸡的使用和试验方案经广东海洋大学滨海农业学院动物福利委员会批准(批准号:SYXK-2018-0147)。

1.2 样品采集

试验结束当日,禁食8 h后,每个重复随机选取1只鸡称重后,翅下采血并分离血清,用于检测血清D-乳酸(D-LA)含量。随后放血屠宰,分离空肠中段2 cm左右固定于4%多聚甲醛,用于末端脱氧核苷酸转移酶介导的dUTP缺口末端标记(TUNEL)法检测肠上皮细胞凋亡;之后纵向剖开空肠,预冷生理盐水清洗后,用灭菌的载玻片刮取黏膜于无酶管中,液氮速冻后,-80 ℃保存,用于相关基因表达分析。

1.3 检测指标及方法

1.3.1 血清D-LA含量

按购于南京建成生物工程研究所的试剂盒说明书测定血清D-LA含量。

1.3.2 荧光定量PCR检测相关基因mRNA表达量

空肠组织RNA提取、cDNA合成及荧光定量PCR方法参照本课题组之前的方法[13],以β-肌动蛋白(β-actin)为内参基因,采用2-ΔΔCt法计算基因mRNA相对表达量[14]。引物序列见表1
表1 引物序列

Table 1 Primer sequences

基因Genes 引物序列Primer sequences (5'—3')
β-肌动蛋白
β-actin
F:ATCCGGACCCTCCATTGTC
R:AGCCATGCCAATCTCGTCTT
闭锁小带蛋白-1
ZO-1
F:CCGCAGTCGTTCACGATCT
R:GGAGAATGTCTGGAATGGTCTGA
闭合蛋白
Occludin
F:GAGCCCAGACTACCAAAGCAA
R:GCTTGATGTGGAAGAGCTTGTTG
密封蛋白-1
Claudin-1
F:ACCCACAGCCTAAGTGCTTC
R:AGGTCTCATAAGGCCCCACT
热休克蛋白70
Hsp70
F:CGTCAGTGCTGTGGACAAGAGTA
R:CCTATCTCTGTTGGCTTCATCCT
热休克蛋白90
Hsp90
F:GAGTTTGACTGACCCGAGCA
R:TCCCTATGCCGGTATCCACA
半胱天冬酶3
Caspase 3
F:CCACCGAGATACCGGACTGT
R:AACTGCTTCGCTTGCTGTGA
半胱天冬酶9
Caspase 9
F:GTGTACCAGCTGCGAGCAGACC
R:GCTTTGAGGTTCCGCAGGGTC
B细胞淋巴瘤-2相关X蛋白
Bax
F:ACTCTGCTGCTGCTCTCCTCTC
R:ATCCACGCAGTGCCAGATGTAATC
B细胞淋巴瘤-2
Bcl-2
F:ATCGTCGCCTTCTTCGAGTT
R:ATCCCATCCTCCGTTGTTCT
Toll样受体4
TLR4
F:CCTGCAACGGTCATCTCAG
R:GTCTCAGGGCTTGTTCTTCAG
核因子-κB p65亚基
NF-κB p65
F:TGAAGAAACGGGAACTGGAAG
R:GGCACGGTTGTCATAGATGG
白细胞介素-1β
IL-1β
F:GCTCTACATGTCGTGTGTGATGAG
R:TGTCGATGTCCCGCATGA
白细胞介素-6
IL-6
F:GCGAGAACAGCATGGAGATG
R:GTAGGTCTGAAAGGCGAACAG
肿瘤坏死因子-α
TNF-α
F:TGTGTATGTGCAGCAACCCGTAGT
R:GGCATTGCAATTTGGACAGAAGT
白细胞介素-10
IL-10
F:AGCTGACGGTGGACCTATTATT
R:GGCTTTGCGCTGGATTC
NOD样受体热蛋白结构域相关蛋白3
NLRP3
F:CCGCTACACCAACCTGACC
R:CACCTGGCCGTCTTTGCT
半胱天冬酶1
Caspase 1
F:CTCTGACAGCACCTTCCT
R:CCGTGGTCCCATTACTCT
白细胞介素-18
IL-18
F:AAGCGTGGCAGCTTTTGAAG
R:CTGAAGGTGCGGTGGTTTTG
核呼吸因子1
NRF1
F:CAGTATAGCACACCTGGTACCCTC
R:CTCCGATGCCTGCGTTGTCT
过氧化物酶体增殖物激活受体γ共激活因子-1α
PGC-1α
F:GATTCTTCACCTGGGTGGCA
R:TCAGCCCGAATTTCCTGGTC
线粒体转录因子A
TFAM
F:GTGAAAGCCTGGCGAAACTG
R:CACAGCTCAGGTTACACCGT
线粒体融合蛋白1
MFN1
F:CCTGCTGCAACTCCAGAGAACAC
R:TCACTCCGCCAACAACGATGATG
线粒体融合蛋白2
MFN2
F:AGCTGGCTGCGTACATCAATGAG
R:GCCTTGCCAACACTTCACTAATGC
视神经萎缩蛋白1
OPA1
F:TGTATGTGATGAGATAGCCTGG
R:CCAGCTCCACTGTACAAGACA
线粒体动力相关蛋白1
DRP1
F:CACGAGACAAGGCTGCTGCTG
R:TTCCTGCTGATACCTCCTCTGC
线粒体裂变因子
MFF
F:GGCTCCTCAGAATGCTGACCTTG
R:CACTACAATCCGCTCTGGAACCTG
PTEN诱导激酶1
PINK1
F:TGCAGTTGTTGGAAGGTGTG
R:CAGCCAGCAGAATCGAACTCTTA
E3泛素连接酶
Parkin
F:GTCCAGCAAAGCATCGTTCA
R:CAACGATGGAAGGATGCTGG
微管相关蛋白1轻链3Ⅰ
LC3Ⅰ
F:TTACACCCATATCAGATTCTTG
R:ATTCCAACCTGTCCCTCA
微管相关蛋白1轻链3Ⅱ
LC3Ⅱ
F:AGTGAAGTGTAGCAGGATGA
R:AAGCCTTGTGAACGAGAT
选择性自噬接头蛋白p62
p62
F:GACCCAGCCAAGACTACCAT
R:CAGAGGCATGTAGTTTCGGC

1.3.3 TUNEL法检测空肠上皮细胞凋亡率

TUNEL法检测空肠上皮细胞凋亡率参照试剂盒说明书进行,在荧光显微镜下进行观察并拍照。每张切片随机选择10个视野,蓝色荧光为正常细胞,绿色荧光为凋亡细胞,采用Image-Pro Plus 6.0软件分别统计阳性和阴性细胞数量,并计算凋亡率。

1.4 数据统计分析

试验数据采用SAS 9.1.3软件进行单因素方差分析,并采用Duncan氏法进行组间差异的显著性比较,结果数据以“平均值±标准误”形式表示,P<0.05表示差异显著。

2 结果

2.1 COS对热应激肉鸡肠道屏障功能的影响

图1所示,HS组肉鸡血清D-LA含量显著高于CON组(P<0.05),HSC-200组血清D-LA含量显著低于HS组(P<0.05)。与CON组相比,HS组空肠闭合蛋白(Occludin)mRNA相对表达量显著降低(P<0.05);与HS组相比,HSC-200组空肠Occludin mRNA相对表达量显著提高(P<0.05)。
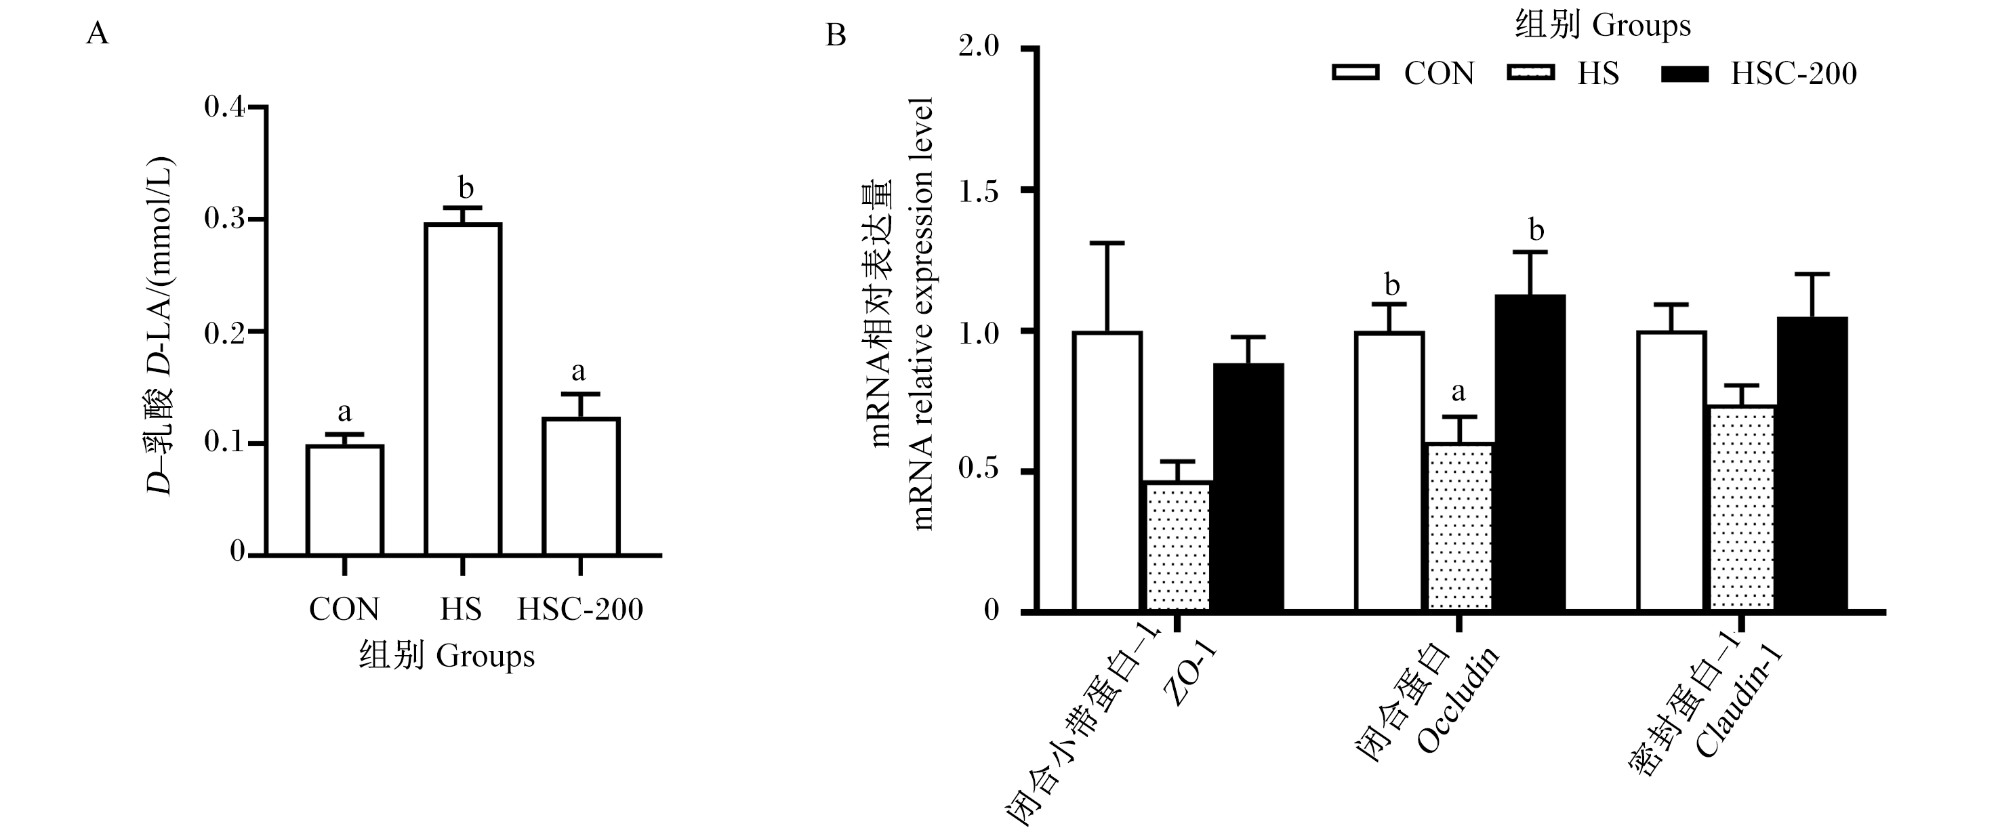
图1 COS对热应激肉鸡肠道屏障功能的影响

数据柱标记不同字母表示差异显著(P<0.05)。下图同。

Fig.1 Effects of COS on intestinal barrier function in heat-stressed broilers

Value columns with different letters indicated significant difference (P<0.05). The same as below.

2.2 COS对热应激肉鸡空肠炎症反应的影响

图2所示,与CON组相比,HS组肉鸡空肠TLR4、核因子-κB p65亚基(NF-κB p65)、白细胞介素-6(IL-6)、NLRP3、半胱天冬酶(Caspase)1和白细胞介素-18(IL-18)mRNA相对表达量显著提高(P<0.05);与HS组相比,HSC-200组空肠TLR4、IL-6、NLRP3、Caspase 1和IL-18 mRNA相对表达量显著降低(P<0.05)。
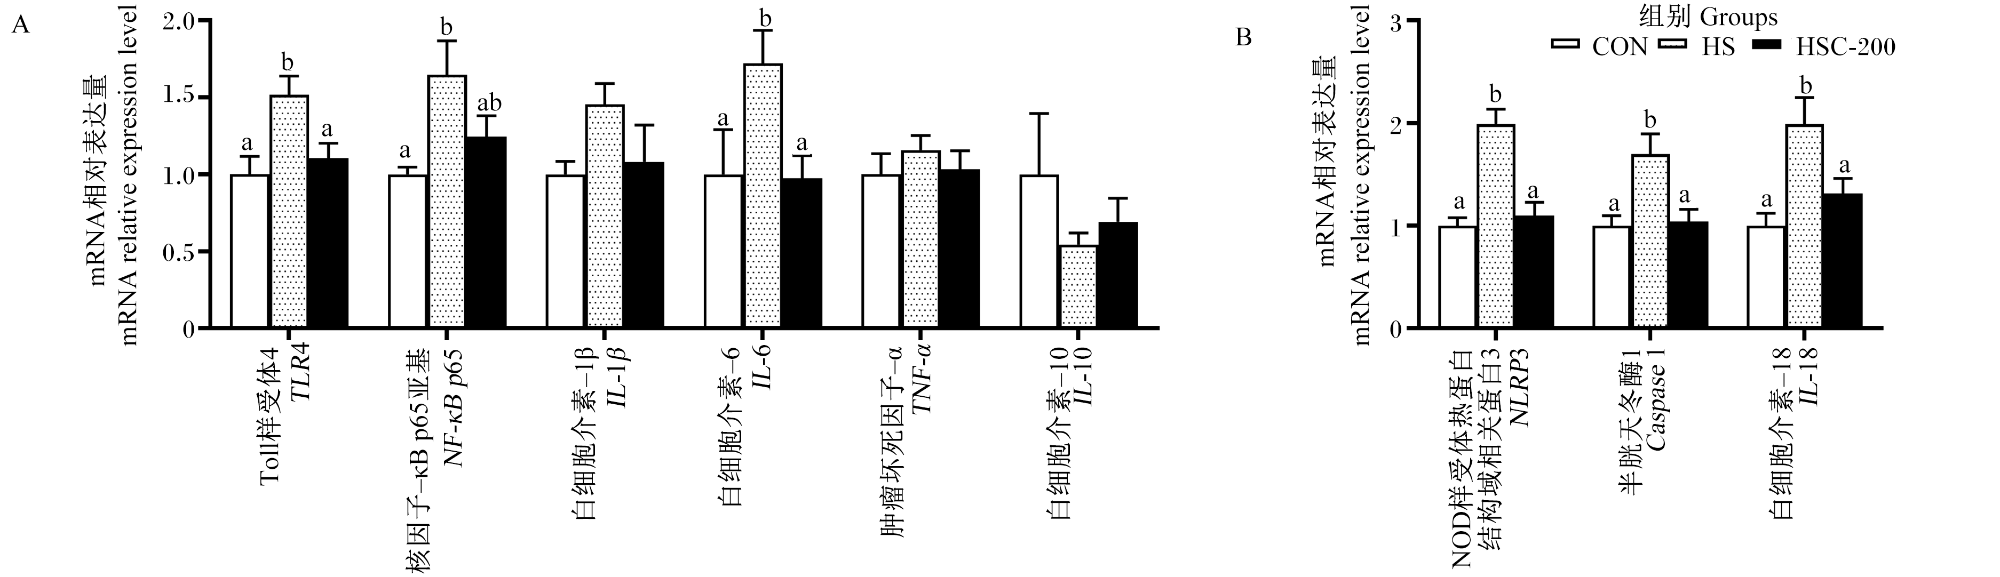
图2 COS对热应激肉鸡空肠炎症反应的影响

Fig.2 Effects of COS on jejunal inflammatory response in heat-stressed broilers

2.3 COS对热应激肉鸡空肠上皮细胞凋亡的影响

图3所示,与CON组相比,HS组肉鸡空肠上皮细胞凋亡率以及热休克蛋白(Hsp)70、Hsp90、Caspase 3和B细胞淋巴瘤-2相关X蛋白(Bax)mRNA相对表达量显著提高(P<0.05),空肠B细胞淋巴瘤-2(Bcl-2)mRNA相对表达量和Bcl-2/Bax值显著降低(P<0.05);与HS组相比,HSC-200组空肠上皮细胞凋亡率以及Hsp70、Hsp90、Caspase 3和Bax mRNA相对表达量显著降低(P<0.05),空肠Bcl-2 mRNA相对表达量和Bcl-2/Bax值显著提高(P<0.05)。
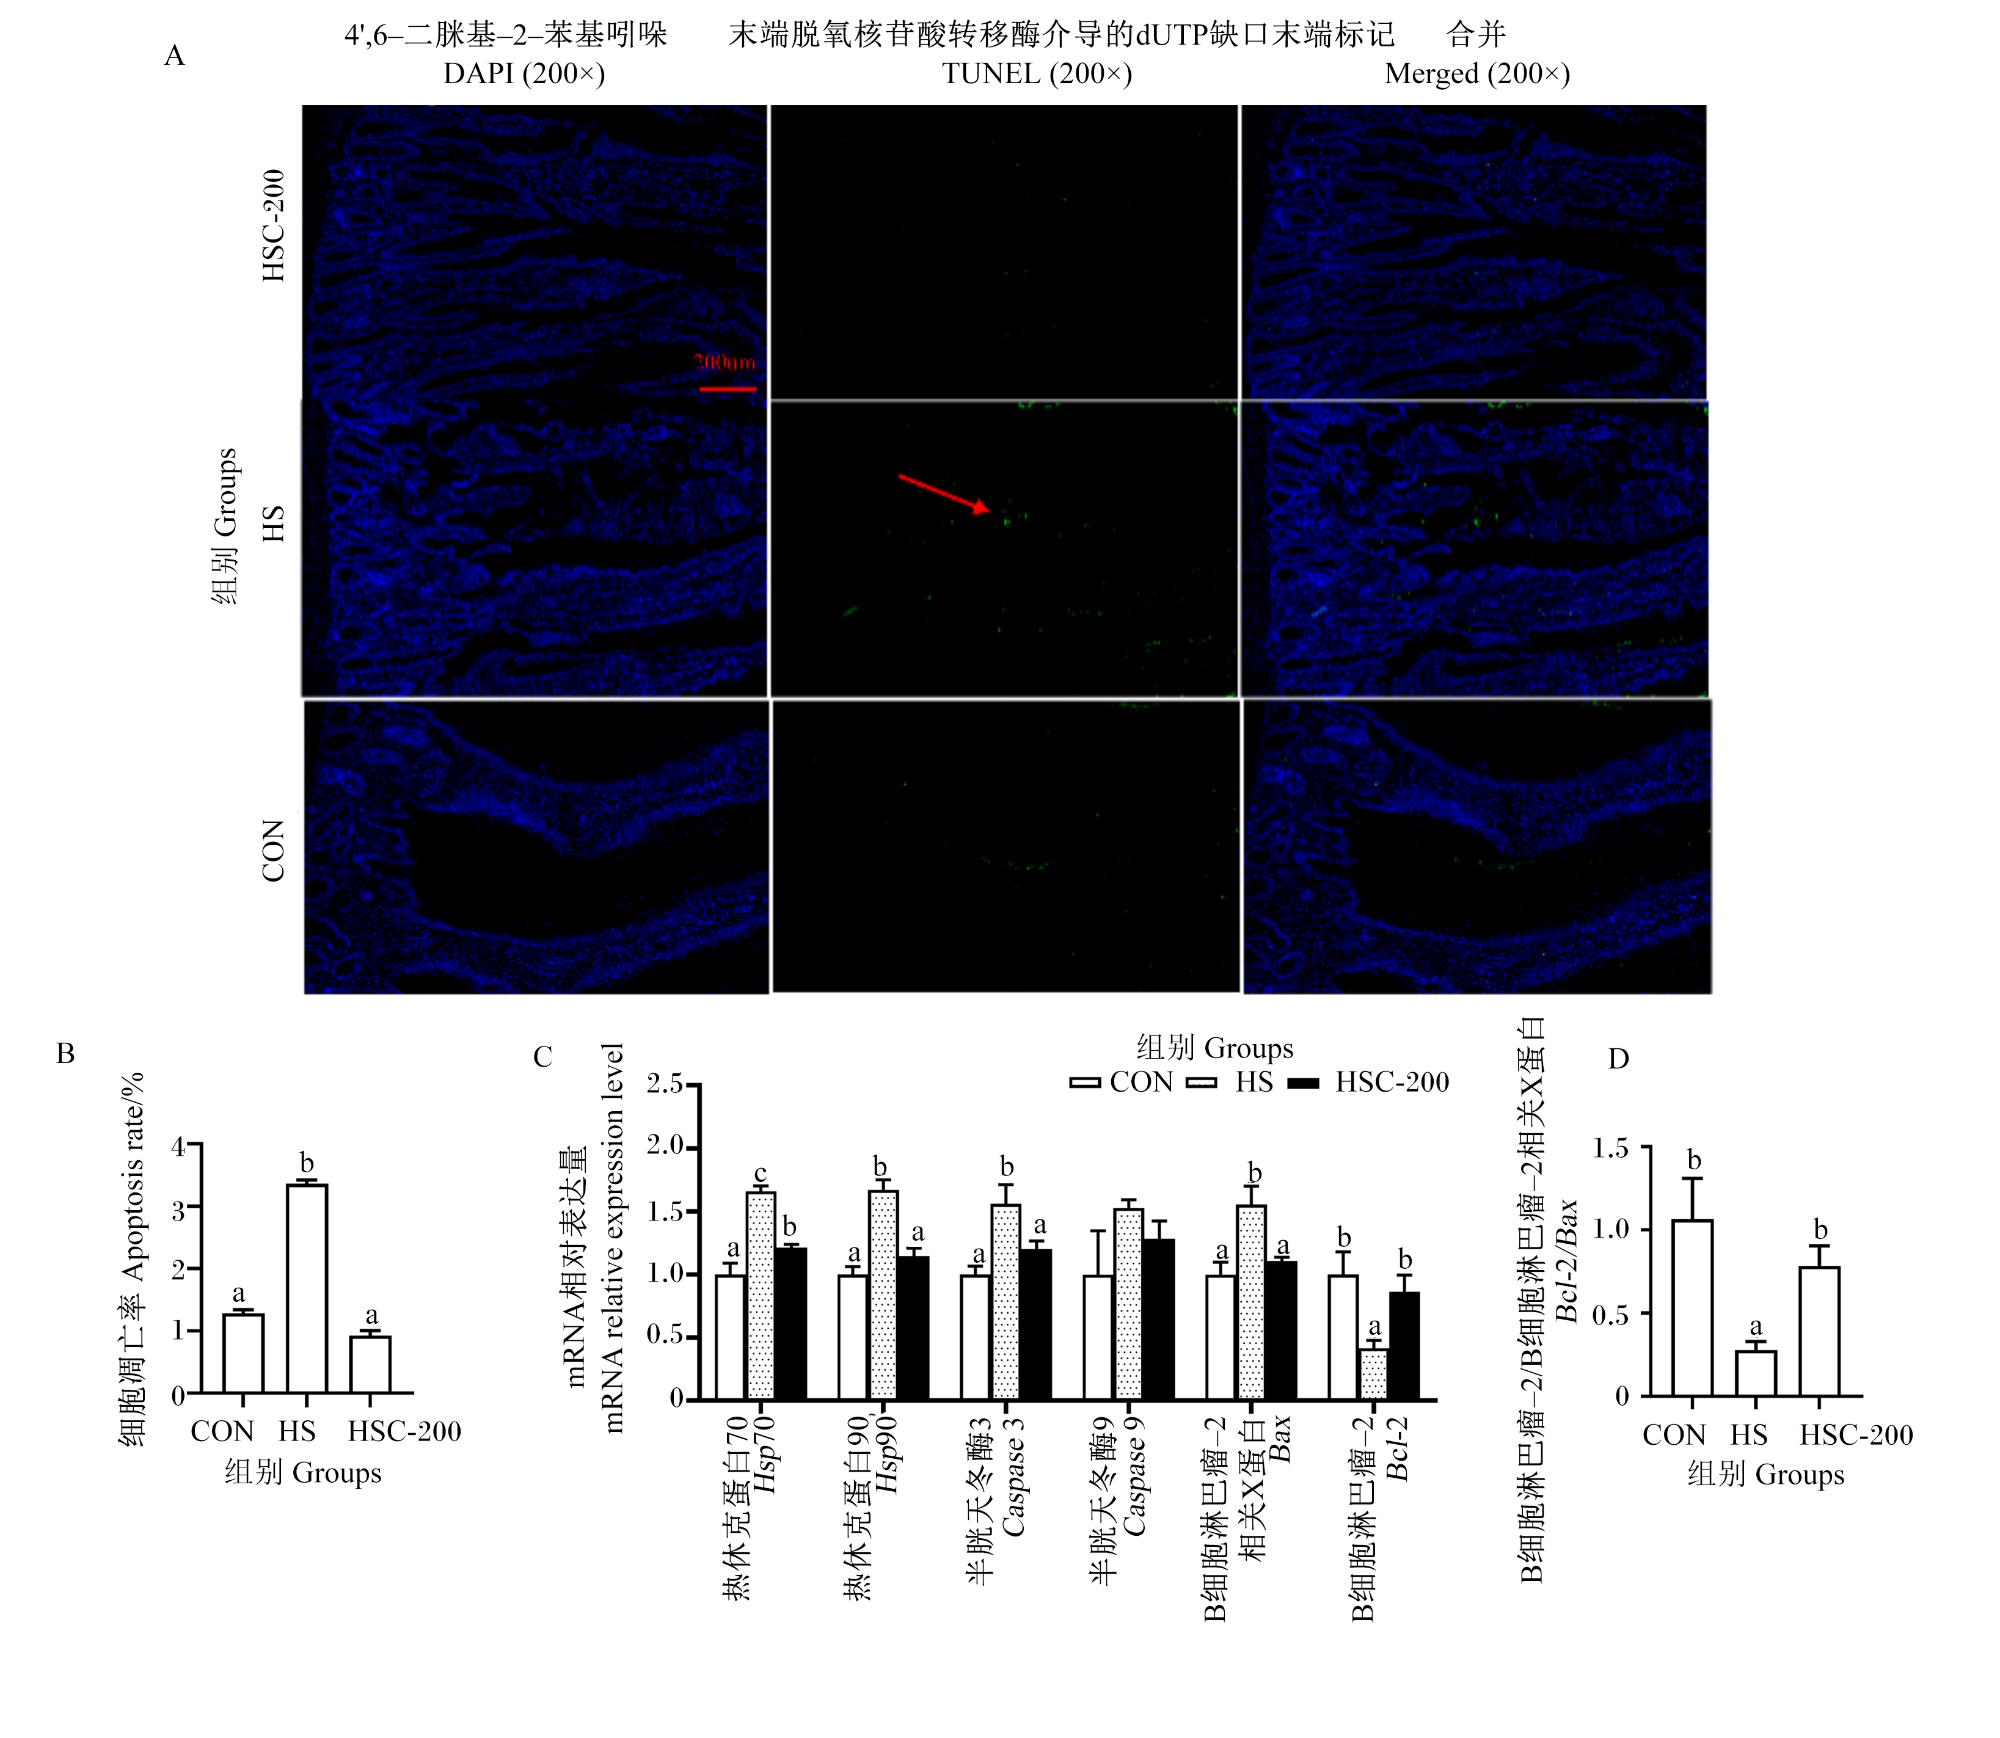
图3 COS对热应激肉鸡空肠上皮细胞凋亡率及凋亡相关基因表达的影响

Fig.3 Effects of COS on jejunal epithelial cell apoptosis rate and apoptosis-related gene expression in heat-stressed broilers

2.4 COS对热应激肉鸡空肠上皮细胞线粒体功能的影响

图4所示,与CON组相比,HS组肉鸡空肠线粒体融合蛋白(MFN)1、MFN2和视神经萎缩蛋白1(OPA1)mRNA相对表达量显著降低(P<0.05),空肠线粒体裂变因子(MFF)、E3泛素连接酶(Parkin)和微管相关蛋白1轻链3Ⅱ(LC3Ⅱ)mRNA相对表达量显著提高(P<0.05);与HS组相比,HSC-200组空肠MFN1和OPA1 mRNA相对表达量显著提高(P<0.05),空肠ParkinLC3Ⅱ mRNA相对表达量显著降低(P<0.05)。
图4 COS对热应激肉鸡空肠上皮细胞线粒体功能的影响

Fig.4 Effects of COS on mitochondrial function of jejunal epithelial cells in heat-stressed broilers

3 讨论

3.1 COS对热应激肉鸡肠道屏障功能的影响

肠上皮细胞不仅是营养物质消化吸收的主要场所,同时肠上皮细胞及其紧密连接蛋白组成的紧密连接也是维持肠道屏障功能的基础[15-16]。紧密连接蛋白主要包括跨膜蛋白密封蛋白(Claudin)-1和Occludin以及支架蛋白闭锁小带蛋白-1(ZO-1)[17]。紧密连接是维持肠道物理屏障功能的重要组成部分,其通透性直接反映肠道屏障功能[18]。本课题组前期研究表明,热应激导致黄羽肉鸡肠道通透性增加,降低十二指肠和空肠相对重量、相对长度、绒毛高度及抗氧化能力[12]。血清D-LA含量是肠道屏障完整性的标志物,与肠道通透性呈正相关[19]。本研究结果显示,热应激提高肉鸡血清D-LA含量,并下调空肠Occludin mRNA相对表达量,表明热应激导致肠道屏障损伤,通透性增加。之前的研究同样表明,热应激下调紧密连接蛋白Claudin-1、Claudin-3、Claudin-4、OccludinZO-1 mRNA相对表达量,并提高血清D-LA含量[20-21]。本课题组前期报道,COS降低氧化应激小鼠血清D-LA含量,并上调空肠ZO-1 mRNA相对表达量[22]。Osho等[23]报道,COS上调地塞米松诱导肉鸡空肠Claudin-1和Occludin mRNA相对表达量。本研究结果同样显示,COS降低热应激肉鸡血清D-LA含量,并上调空肠Occludin mRNA相对表达量,表明COS能缓解热应激导致的肠道屏障损伤,这可能与COS的抗氧化和抗炎功能相关[12]

3.2 COS对热应激肉鸡肠道炎症反应的影响

本课题组前期研究报道,热应激导致肉鸡肠道氧化损伤[3,12]。氧化损伤促进炎症的发生和细胞凋亡[24]。热应激激活TLR4/NF-κB炎症信号通路,增加促炎因子的成熟和分泌[25]。此外,热应激还可以直接或间接激活NLRP3炎症小体,通过活化Caspase 1,增加促炎因子白细胞介素-1β(IL-1β)和IL-18的成熟和分泌,加剧肠道炎性损伤[26-27]。Lan等[12]报道,热应激提高肉鸡十二指肠和空肠IL-1β以及空肠肿瘤坏死因子-α(TNF-α)含量。欧阳经鑫等[27]报道,热应激上调肉鸡空肠IL-1βTNF-αNLRP3和IL-18及回肠IL-1βTNF-αNLRP3和Caspase 1 mRNA相对表达量。Liu等[5]报道,热应激上调肉鸡回肠NF-κB p65、IL-1βTNF-α mRNA相对表达量。本试验结果同样表明,热应激上调肉鸡空肠TLR4、NF-κB p65、IL-6、NLRP3、Caspase 1和IL-18 mRNA相对表达量,表明热应激损伤肠道屏障功能,且与炎症通路的激活和促炎因子的释放相关。Lan等[12]报道,COS通过降低热应激肉鸡十二指肠和空肠IL-1β含量,缓解肠道屏障损伤。Hu等[28]报道,COS通过下调IL-6、TNF-αNLRP3、Caspase 1和IL-18 mRNA相对表达量,缓解巨噬细胞的炎症反应。本试验结果同样表明,COS下调热应激肉鸡空肠TLR4、IL-6、NLRP3、Caspase 1和IL-18 mRNA相对表达量,表明COS可能通过抑制TLR4/NF-κB信号通路和NLRP3炎症小体的活化,下调促炎因子的表达以缓解热应激肉鸡空肠的炎性损伤。

3.3 COS对热应激肉鸡肠上皮细胞凋亡的影响

热应激诱导的氧化损伤和炎症反应会导致细胞凋亡[29]。凋亡是细胞的一种程序化死亡方式,肠上皮细胞在凋亡与增殖之间保持动态平衡,细胞的过度凋亡导致肠道屏障损伤。为了阐明COS缓解热应激肉鸡肠道屏障损伤是否与细胞凋亡相关,本试验检测了空肠上皮细胞的凋亡率和线粒体凋亡相关因子基因的表达变化,结果表明,热应激显著提高肉鸡空肠上皮细胞凋亡率,并上调空肠Hsp70、Hsp90、Caspase 3和Bax mRNA相对表达量,下调空肠Bcl-2 mRNA相对表达量和Bcl-2/Bax值,表明热应激可能通过上调促凋亡因子(Caspase 3和Bax)、下调抗凋亡因子(Bcl-2)mRNA相对表达量诱导空肠上皮细胞凋亡,损伤肠道屏障。体外研究发现,热应激通过激活线粒体凋亡相关因子诱导猪肾小管上皮细胞凋亡[30],此外,热应激显著提高肉鸡肝脏、十二指肠、胸腺、脾脏和法氏囊细胞凋亡率[5,31-32]。分子伴侣蛋白Hsp70和Hsp90有抗应激和抗凋亡的作用,热应激能上调Hsp70和Hsp90 mRNA相对表达量,通过线粒体途径调控细胞凋亡[33]。Wang等[34]报道,热应激上调肉鸡法氏囊Caspase 3和Bax蛋白表达,并下调法氏囊和胸腺Bcl-2蛋白表达。Mo等[35]报道,热应激上调小鼠空肠Caspase 3和Bax蛋白表达以及Bax/Bcl-2值,并下调空肠Bcl-2蛋白表达。Shi等[36]报道,热应激上调肉鸡空肠Hsp90和Bax mRNA相对表达量,并下调Bcl-2 mRNA相对表达量。Guo等[37]报道,COS降低溃疡性结肠炎小鼠的结肠上皮细胞凋亡率。Tao等[38]报道,COS下调脂肪肝综合征蛋鸡卵巢Caspase 9 mRNA相对表达量,并上调Bcl-2 mRNA相对表达量。Meng等[39]报道,COS下调脂多糖(LPS)诱导断奶仔猪空肠和回肠Caspase 3含量,并下调空肠Bax mRNA相对表达量。本研究结果同样表明,COS降低热应激肉鸡空肠上皮细胞凋亡率,下调空肠Hsp70、Hsp90、Caspase 3和Bax mRNA相对表达量,上调空肠Bcl-2 mRNA相对表达量和Bcl-2/Bax值,表明COS可能通过缓解热应激肉鸡肠上皮细胞凋亡缓解肠道屏障损伤。COS缓解热应激肉鸡肠上皮细胞凋亡,可能与COS的抗氧化和抗炎功能相关[11]

3.4 COS对热应激肉鸡肠上皮细胞线粒体功能的影响

热应激除了能直接损伤线粒体功能,其诱导的氧化损伤和炎症反应也会损伤线粒体功能,进而诱导线粒体凋亡相关因子的表达,最终导致细胞凋亡[29,36]。线粒体功能稳定主要与线粒体动力学相关,即通过维持线粒体生物发生、融合和分裂的动态平衡来维持其生理功能和细胞内稳态[8]。线粒体生物合成本质是为了提升线粒体的数量和质量,核呼吸因子1(NRF1)、过氧化物酶体增殖物激活受体γ共激活因子-1α(PGC-1α)和线粒体转录因子A(TFAM)与线粒体的生物发生密切相关[40]。线粒体融合受MFN1、MFN2和OPA1的调节,线粒体分裂主要由线粒体动力相关蛋白1(DRP1)和MFF调节[41]。线粒体的融合和分裂不平衡,会使线粒体的形态和数目发生改变,同时诱发线粒体损伤和细胞凋亡[42]。杨泰[43]报道,热应激下调肉鸡空肠和回肠NRF1、PGC-1αTFAM mRNA相对表达量,导致线粒体损伤和功能障碍。Zeng等[29]报道,热应激上调牛乳腺上皮细胞DRP1 mRNA相对表达量,下调MFN1和MFN2 mRNA相对表达量,导致线粒体功能损伤以及细胞氧化应激和凋亡。本研究结果同样表明,热应激下调肉鸡空肠MFN1、MFN2和OPA1 mRNA相对表达量,上调空肠MFF mRNA相对表达量,表明热应激破坏肉鸡空肠上皮细胞线粒体分裂和融合的动态平衡,导致线粒体功能损伤和细胞凋亡。关于COS对线粒体分裂和融合的调节作用还未见相关报道,但Liu等[44]报道,木聚糖上调LPS诱导断奶仔猪空肠MFN1 mRNA相对表达量,下调空肠DRP1 mRNA相对表达量,表明寡糖能参与调节线粒体的分裂与融合。此外,藻酸寡糖和巴戟天寡糖也被证实对线粒体的功能有积极作用[45-46]。本研究结果显示,COS上调热应激肉鸡空肠MFN1和OPA1 mRNA相对表达量,表明COS可能通过促进热应激肉鸡空肠上皮细胞线粒体的融合,减少受损线粒体的数量,以维持线粒体分裂和融合的动态平衡,这可能是COS改善线粒体功能的关键机制之一。
肠道屏障损伤与细胞凋亡和线粒体自噬密切相关[47]。线粒体自噬是选择性清除受损线粒体以维持细胞正常功能,与线粒体生物发生、分裂和融合密切相关[9]。热应激损伤线粒体功能,使得膜电位下降,招募PTEN诱导激酶1(PINK1)到线粒体膜上,结合并激活Parkin,由选择性自噬接头蛋白p62协助与LC3Ⅱ结合,最终诱导线粒体自噬[48]。肠上皮细胞自噬失调是肠道炎性损伤和细胞凋亡的主要诱因,线粒体自噬抑制或过度激活,会促发ATP合成受阻、线粒体膜电位下降、ROS过度释放等级联反应,激活TLR4/NF-κB和NLRP3炎症信号通路,促进促炎因子的释放并导致细胞凋亡,最终损伤肠道屏障[6,10,49]。Cao等[50]报道,氧化应激通过过度激活PINK1-Parkin线粒体自噬通路,导致IPEC-J2细胞线粒体功能和屏障损伤。热应激导致的肠道屏障损伤是否也与线粒体过度自噬相关?本研究结果表明,热应激提高肉鸡空肠ParkinLC3Ⅱ mRNA相对表达量,表明热应激过度激活空肠线粒体的自噬进而导致屏障损伤。对软骨细胞和骨肉瘤细胞的研究发现,COS能通过调节线粒体自噬缓解炎性损伤[51-52]。本试验结果同样表明,COS能通过下调肉鸡空肠ParkinLC3Ⅱ mRNA相对表达量,以缓解热应激肉鸡空肠线粒体的过度自噬。以上研究结果表明,COS可能通过改善热应激肉鸡线粒体的功能来缓解肠道屏障损伤。但值得注意的是,COS缓解热应激肉鸡空肠线粒体的过度自噬,是COS的直接作用?还是由于COS促进热应激肉鸡空肠上皮细胞线粒体的融合,减少受损线粒体的数量,维持线粒体分裂和融合的动态平衡,进而降低了自噬水平?亦或是二者的协同作用,这还不明确,仍需做进一步研究。

4 结论

COS通过改善热应激肉鸡肠上皮细胞线粒体功能,进而缓解炎症反应,减少细胞凋亡,最终发挥保护肠道屏障的作用。
[1]
APALOWO O O, EKUNSEITAN D A, FASINA Y O. Impact of heat stress on broiler chicken production[J]. Poultry, 2024, 3(2):107-128.

DOI

[2]
KHAN R U, NAZ S, ULLAH H, et al. Physiological dynamics in broiler chickens under heat stress and possible mitigation strategies[J]. Animal Biotechnology, 2023, 34(2):438-447.

DOI

[3]
张迦, 王浩轩, 高金稔, 等. 壳寡糖对热应激肉鸡生长性能及肠道消化吸收功能的影响[J]. 动物营养学报, 2025, 37(7):4408-4421.

DOI

ZHANG J, WANG H X, GAO J R, et al. Effects of chitosan oligosaccharides on growth performance and intestinal digestion and absorption function of broilers under heat stress[J]. Chinese Journal of Animal Nutrition, 2025, 37(7):4408-4421. (in Chinese)

DOI

[4]
BRUGALETTA G, TEYSSIER J R, ROCHELL S J, et al. A review of heat stress in chickens.Part Ⅰ:insights into physiology and gut health[J]. Frontiers in Physiology, 2022, 13:934381.

DOI

[5]
LIU W C, ZHU Y R, ZHAO Z H, et al. Effects of dietary supplementation of algae-derived polysaccharides on morphology,tight junctions,antioxidant capacity and immune response of duodenum in broilers under heat stress[J]. Animals, 2021, 11(8):2279.

DOI

[6]
罗烨, 刘慧敏, 瞿明仁, 等. 热应激诱导炎症反应及细胞自噬的调控机制[J]. 动物营养学报, 2024, 36(10):6191-6200.

DOI

LUO Y, LIU H M, QU M R, et al. Regulatory mechanism of heat stress-induced inflammatory response and autophagy[J]. Chinese Journal of Animal Nutrition, 2024, 36(10):6191-6200. (in Chinese)

DOI

[7]
NUNNARI J, SUOMALAINEN A. Mitochondria:in sickness and in health[J]. Cell, 2012, 148(6):1145-1159.

DOI

[8]
MARZETTI E, CSISZAR A, DUTTA D, et al. Role of mitochondrial dysfunction and altered autophagy in cardiovascular aging and disease:from mechanisms to therapeutics[J]. American Journal of Physiology:Heart and Circulatory Physiology, 2013, 305(4):H459-H476.

[9]
LENIN R R, KOH Y H, ZHANG Z T, et al. Dysfunctional autophagy,proteostasis,and mitochondria as a prelude to age-related macular degeneration[J]. International Journal of Molecular Sciences, 2023, 24(10):8763.

DOI

[10]
杨攀, 方梦瑶, 田志梅, 等. 线粒体自噬与免疫稳态、肠道健康的互联机制及其调控研究进展[J]. 动物营养学报, 2025, 37(3):1424-1435.

DOI

YANG P, FANG M Y, TIAN Z M, et al. Research progress on interconnected mechanisms of mitophagy with immune homeostasis and gut health and its regulation[J]. Chinese Journal of Animal Nutrition, 2025, 37(3):1424-1435. (in Chinese)

DOI

[11]
LI Q Y, SHI W R, HUANG Y L. Comparison of the protective effects of chitosan oligosaccharides and chitin oligosaccharide on apoptosis,inflammation and oxidative stress[J]. Experimental and Therapeutic Medicine, 2024, 28(2):310.

DOI

[12]
LAN R X, LI Y X, CHANG Q Q, et al. Dietary chitosan oligosaccharides alleviate heat stress-induced intestinal oxidative stress and inflammatory response in yellow-feather broilers[J]. Poultry Science, 2020, 99(12):6745-6752.

DOI PMID

[13]
LAN R X, LIU F, HE Z B, et al. Immunolocalization of GnRHRI,gonadotropin receptors,PGR,and PGRMCI during follicular development in the rabbit ovary[J]. Theriogenology, 2014, 81(8):1139-1147.

DOI

[14]
LIVAK K J, SCHMITTGEN T D. Analysis of relative gene expression data using real-time quantitative PCR and the 2-ΔΔCT method[J]. Methods, 2001, 25(4):402-408.

DOI

[15]
ZHANG Q Y, ZHANG S, WU S, et al. Supplementing the early diet of broilers with soy protein concentrate can improve intestinal development and enhance short-chain fatty acid-producing microbes and short-chain fatty acids,especially butyric acid[J]. Journal of Animal Science and Biotechnology, 2022, 13(1):97.

DOI

[16]
DU E C, JIANG M H, CHEN F, et al. Dietary honokiol supplementation improves antioxidant capacity,enhances intestinal health,and modulates cecal microbial composition and function of broiler chickens[J]. Poultry Science, 2024, 103(7):103798.

DOI

[17]
OTANI T, FURUSE M. Tight junction structure and function revisited[J]. Trends in Cell Biology, 2020, 30(10):805-817.

DOI PMID

[18]
HOROWITZ A, CHANEZ-PAREDES S D, HAEST X, et al. Paracellular permeability and tight junction regulation in gut health and disease[J]. Nature Reviews Gastroenterology & Hepatology, 2023, 20(7):417-432.

[19]
CHEN S Y, XUE Y J, SHEN Y T, et al. Effects of different selenium sources on duodenum and jejunum tight junction network and growth performance of broilers in a model of fluorine-induced chronic oxidative stress[J]. Poultry Science, 2022, 101(3):101664.

DOI

[20]
ALHOTAN R A, AL SULAIMAN A R, ALHARTHI A S, et al. Protective influence of betaine on intestinal health by regulating inflammation and improving barrier function in broilers under heat stress[J]. Poultry Science, 2021, 100(9):101337.

DOI

[21]
OUYANG J X, ZHANG C, DENG C X, et al. Dietary vitamin B6 supplementation alleviates heat stress-induced intestinal barrier impairment by regulating the gut microbiota and metabolites in broilers[J]. Poultry Science, 2024, 103(11):104202.

DOI

[22]
LAN R X, CHANG Q Q, WEI L L, et al. The protect effects of chitosan oligosaccharides on intestinal integrity by regulating oxidative status and inflammation under oxidative stress[J]. Marine Drugs, 2021, 19(2):57.

DOI

[23]
OSHO S O, ADEOLA O. Chitosan oligosaccharide supplementation alleviates stress stimulated by in-feed dexamethasone in broiler chickens[J]. Poultry Science, 2020, 99(4):2061-2067.

DOI PMID

[24]
XIA Y, LUO Q H, HUANG C, et al. Ferric citrate-induced colonic mucosal damage associated with oxidative stress,inflammation responses,apoptosis,and the changes of gut microbial composition[J]. Ecotoxicology and Environmental Safety, 2023, 249:114364.

DOI

[25]
TANG L P, LI W H, LIU Y L, et al. Heat stress aggravates intestinal inflammation through TLR4-NF-κB signaling pathway in Ma chickens infected with Escherichia coli O157:H7[J]. Poultry Science, 2021, 100(5):101030.

DOI

[26]
ZHOU R B, YAZDI A S, MENU P, et al. A role for mitochondria in NLRP3 inflammasome activation[J]. Nature, 2011, 469(7329):221-225.

DOI

[27]
欧阳经鑫, 李秋粉, 周华, 等. 饲粮添加色氨酸对热应激肉鸡肝脏、肠道抗氧化能力和炎症反应的影响[J]. 中国兽医学报, 2022, 42(6):1256-1262,1269.

OUYANG J X, LI Q F, ZHOU H, et al. Effects of dietary tryptophan supplementation on antioxidant capacity and inflammatory response in liver and intestine of broilers subjected to heat stress[J]. Chinese Journal of Veterinary Science, 2022, 42(6):1256-1262,1269. (in Chinese)

[28]
HU H M, XIA H, ZOU X J, et al. N-acetyl-chitooligosaccharide attenuates inflammatory responses by suppression of NF-κB signaling,MAPK and NLRP3 inflammasome in macrophages[J]. Journal of Functional Foods, 2021, 78:104364.

DOI

[29]
ZENG H F, XU J, WANG X L, et al. Nicotinamide mononucleotide alleviates heat stress-induced oxidative stress and apoptosis in BMECs through reducing mitochondrial damage and endoplasmic reticulum stress[J]. Ecotoxicology and Environmental Safety, 2022, 235:113441.

DOI

[30]
霍爱华, 孙雪荣, 于文慧, 等. 热应激诱导猪肾小管上皮(LLC-PK1)细胞线粒体凋亡相关因子的时效表达[J]. 华北农学报, 2016, 31(6):94-99.

DOI

HUO A H, SUN X R, YU W H, et al. Expression of factors related to mitochondrial apoptosis in pig kidney proximal tubular (LLC-PK1) cells induced by heat stress[J]. Acta Agriculturae Boreali-Sinica, 2016, 31(6):94-99. (in Chinese)

DOI

[31]
MA B B, XING T, LI J L, et al. Chronic heat stress causes liver damage via endoplasmic reticulum stress-induced apoptosis in broilers[J]. Poultry Science, 2022, 101(10):102063.

DOI

[32]
MAO Y, KONG X Y, LIANG Z G N, et al. Viola yedoensis Makino alleviates heat stress-induced inflammation,oxidative stress,and cell apoptosis in the spleen and thymus of broilers[J]. Journal of Ethnopharmacology, 2024, 319(Pt 3):117350.

DOI

[33]
CEDRAZ H, GROMBONI J G G, PINTO GARCIA A A Junior, et al. Heat stress induces expression of HSP genes in genetically divergent chickens[J]. PLoS One, 2017, 12(10):e0186083.

DOI

[34]
WANG D C, HU F J, LIU H, et al. Effects of chicken hemoglobin antimicrobial peptides on intestinal mucosal immunity under chronic heat stress and vaccination responses in broilers[J]. Frontiers in Veterinary Science, 2025, 12:1574513.

DOI

[35]
MO F, QIN X Y, ZHOU X, et al. Trehalose supplementation ameliorates heat stress-induced intestinal barrier dysfunction by suppressing endoplasmic reticulum stress and modulating gut microbiota in mice[J]. The Journal of Nutritional Biochemistry, 2025, 146:110065.

DOI

[36]
SHI H, ZHANG J Q, LIU H J, et al. Dietary rutin improves growth performance,intestinal barrier,mitochondrial homeostasis and redox balance in broilers under heat stress[J]. Italian Journal of Animal Science, 2025, 24(1):1573-1585.

DOI

[37]
GUO J, LIAO M F, ZHU Y J, et al. The protective role of chitooligosaccharides against chronic ulcerative colitis induced by dextran sulfate sodium in mice[J]. Journal of Functional Foods, 2021, 87:104809.

DOI

[38]
TAO W J, JIN F, FAN Q W, et al. Effects of chitosan oligosaccharide on production performance,egg quality and ovarian function in laying hens with fatty liver syndrome[J]. Animals, 2022, 12(18):2465.

DOI

[39]
MENG T T, LIU C M, CHEN Y L, et al. Dietary chito-oligosaccharide attenuates LPS-challenged intestinal inflammation via regulating mitochondrial apoptotic and MAPK signaling pathway[J]. International Immunopharmacology, 2024, 126:111153.

DOI

[40]
SCARPULLA R C. Transcriptional paradigms in mammalian mitochondrial biogenesis and function[J]. Physiological Reviews, 2008, 88(2):611-638.

DOI PMID

[41]
FRIEDMAN J R, NUNNARI J. Mitochondrial form and function[J]. Nature, 2014, 505(7483):335-343.

DOI

[42]
BI J B, ZHANG J, REN Y F, et al. Irisin alleviates liver ischemia-reperfusion injury by inhibiting excessive mitochondrial fission,promoting mitochondrial biogenesis and decreasing oxidative stress[J]. Redox Biology, 2019, 20:296-306.

DOI

[43]
杨泰. 鞣花酸对热应激肉鸡肠道损伤保护效应及机制研究[D]. 博士学位论文. 长沙: 湖南农业大学, 2022:70.

YANG T. Study on the protective effect and mechanism of ellagic acid on intestinal damage in heat-stressed broiler chickens[D]. Ph.D. Thesis. Changsha: Hunan Agricultural University, 2022:70. (in Chinese)

[44]
LIU G M, SUN W X, ZHANG R N, et al. Dietary xylo-oligosaccharides alleviates LPS-induced intestinal injury via endoplasmic reticulum-mitochondrial system pathway in piglets[J]. Journal of Animal Science, 2024, 102:skae238.

DOI

[45]
FENG W J, LIU J Y, WANG S, et al. Alginate oligosaccharide alleviates D-galactose-induced cardiac ageing via regulating myocardial mitochondria function and integrity in mice[J]. Journal of Cellular and Molecular Medicine, 2021, 25(15):7157-7168.

DOI

[46]
WANG X L, JIANG H, ZHANG N, et al. Anti-diabetic activities of agaropectin-derived oligosaccharides from Gloiopeltis furcata via regulation of mitochondrial function[J]. Carbohydrate Polymers, 2020, 229:115482.

DOI

[47]
ZHANG J J, WANG J Q, XU X Y, et al. Red ginseng protects against cisplatin-induced intestinal toxicity by inhibiting apoptosis and autophagy via the PI3K/AKT and MAPK signaling pathways[J]. Food & Function, 2020, 11(5):4236-4248.

[48]
YIN K L, LEE J, LIU Z L, et al. Mitophagy protein PINK1 suppresses colon tumor growth by metabolic reprogramming via p53 activation and reducing acetyl-CoA production[J]. Cell Death and Differentiation, 2021, 28(8):2421-2435.

DOI PMID

[49]
GAO D L, LIN M R, GE N, et al. From macroautophagy to mitophagy:unveiling the hidden role of mitophagy in gastrointestinal disorders[J]. World Journal of Gastroenterology, 2024, 30(23):2934-2946.

DOI

[50]
CAO S T, XIAO H, LI X, et al. AMPK-PINK1/parkin mediated mitophagy is necessary for alleviating oxidative stress-induced intestinal epithelial barrier damage and mitochondrial energy metabolism dysfunction in IPEC-J2[J]. Antioxidants, 2021, 10(12):2010.

DOI

[51]
PAN Z, CHENG D D, WEI X J, et al. Chitooligosaccharides inhibit tumor progression and induce autophagy through the activation of the p53/mTOR pathway in osteosarcoma[J]. Carbohydrate Polymers, 2021, 258:117596.

DOI

[52]
CAO R Q, YU H M, LONG H B, et al. Low deacetylation degree chitosan oligosaccharide protects against IL-1β induced inflammation and enhances autophagy activity in human chondrocytes[J]. Journal of Biomaterials Science Polymer Edition, 2022, 33(4):517-531.

DOI

文章导航

/