综述

功能性脂肪酸通过微生物-肠-脑轴对畜禽繁殖性能的影响及调控机制研究进展

  • 梁馨月 , 1, 2 ,
  • 翟双双 2 ,
  • 蒋守群 1 ,
  • 阮栋 , 1, *
展开
  • 1 广东省农业科学院动物科学研究所, 猪禽种业国家重点实验室,农业农村部华南动物营养与饲料重点实验室,广东省畜禽育种与营养重点实验室, 广州 510640
  • 2 长江大学, 动物科学技术学院, 荆州 430100
*阮 栋,研究员,硕士生导师,E-mail:

梁馨月(2002—),女,湖北恩施人,硕士研究生,研究方向为动物营养与饲料科学。E-mail:

Office editor: 武海龙

收稿日期: 2025-09-10

  网络出版日期: 2026-05-14

基金资助

广东省饲料产业技术体系(2024CXTD14)

国家肉鸡产业技术体系项目(CARS-41-G10)

国家重点研发专项(2021YFD300404)

广东省科技计划项目(2023A0505050104)

广州市科技计划项目(2024E04J0562)

广州市科技计划项目(202206010168)

Research Process on Effects and Regulatory Mechanism of Functional Fatty Acids on Reproductive Performance of Livestock and Poultry via Microbial-Gut-Brain Axis

  • LIANG Xinyue , 1, 2 ,
  • ZHAI Shuangshuang 2 ,
  • JIANG Shouqun 1 ,
  • RUAN Dong , 1, *
Expand
  • 1 Guangdong Provincial Key Laboratory of Animal Breeding and Nutrition, Key Laboratory of Animal Nutrition and Feed Science in South China, Ministry of Agriculture and Rural Affairs, State Key Laboratory of Swine and Poultry Breeding, Institute of Animal Science, Guangdong Academy of Agricultural Sciences, Guangzhou 510640, China
  • 2 College of Animal Science and Technology, Yangtze University, Jingzhou 430100, China
*professor, E-mail:

Received date: 2025-09-10

  Online published: 2026-05-14

摘要

功能性脂肪酸作为一类具有抗氧化、抗炎和免疫调节功能的生物活性分子,在畜禽生殖生理调控中发挥着关键作用。功能性脂肪酸通过调节肠道菌群结构,经血液循环、神经递质、迷走神经等通路对类固醇激素生成、卵泡发育、乳腺发育、睾酮合成及精子品质等生理过程进行调控,以及对G蛋白偶联受体、磷脂酰肌醇3-激酶和丝裂原活化蛋白激酶等信号通路进行调控,进而增强畜禽繁殖性能。其代谢途径与作用机制包括肠道菌群调控、微生物-肠-脑轴信号传递及机体免疫与代谢稳态调节。本文旨在揭示功能性脂肪酸对畜禽繁殖性能的影响及调控机制,优化饲料营养调控措施,以提高畜禽繁殖力、改善子代健康,为畜禽高效健康养殖和绿色可持续发展提供科学依据。

本文引用格式

梁馨月 , 翟双双 , 蒋守群 , 阮栋 . 功能性脂肪酸通过微生物-肠-脑轴对畜禽繁殖性能的影响及调控机制研究进展[J]. 动物营养学报, 2026 , 38(5) : 3280 -3291 . DOI: 10.12418/CJAN2026.262

Abstract

Functional fatty acids, as bioactive molecules with antioxidant, anti-inflammatory and immunomodulatory properties, play a crucial role in regulating reproductive physiology in livestock and poultry. Functional fatty acids regulate the intestinal flora structure, modulate physiological processes including steroid hormone production, follicular development, mammary gland growth, testosterone synthesis and sperm quality through blood circulation, neurotransmitters and vagus nerve pathways, and modulate the signaling pathways including G protein-coupled receptors, phosphatidylinositol 3-kinase and mitogen-activated protein kinase, and then enhance the reproductive performance of livestock and poultry. Their metabolic pathways and mechanisms include gut microbiota regulation, microbial-gut-brain axis signaling and immune and metabolic homeostasis modulation. This study aims to elucidate the effects of functional fatty acids on reproductive performance of livestock and poultry, optimize feed nutrition strategies to improve breeding efficiency and offspring health, and provide scientific evidence for efficient, healthy farming practices and sustainable development in animal husbandry.

功能性脂肪酸是一类具有特定生物学效应的脂肪酸,不仅作为能量来源并参与细胞膜构成,还具备抗炎[1]及免疫调节[2]等功能。功能性脂肪酸根据碳链长度、饱和度以及双键位置分为多个类别,主要包括短链脂肪酸(short-chain fatty acids,SCFA),如乙酸、丙酸、丁酸等;中链脂肪酸(medium chain fatty acids,MCFA),如葵酸、月桂酸、辛酸等;以及长链多不饱和脂肪酸(polyunsaturated fatty acids,PUFA),如ω-3和ω-6 PUFA等。这些脂肪酸的来源可通过膳食补充、微生物合成及体内代谢转化等途径,参与调节家禽机体的多种生理过程。目前,关于功能性脂肪酸通过微生物-肠-脑轴对畜禽的繁殖调控是近年来畜牧领域的研究热点。因此,本文就功能性脂肪酸的生物学功能、作用机制等进行综述,为其在畜禽养殖与饲料生产上的研究与应用提供参考。

1 功能性脂肪酸概述

1.1 功能性脂肪酸的来源、常见类型及化学结构
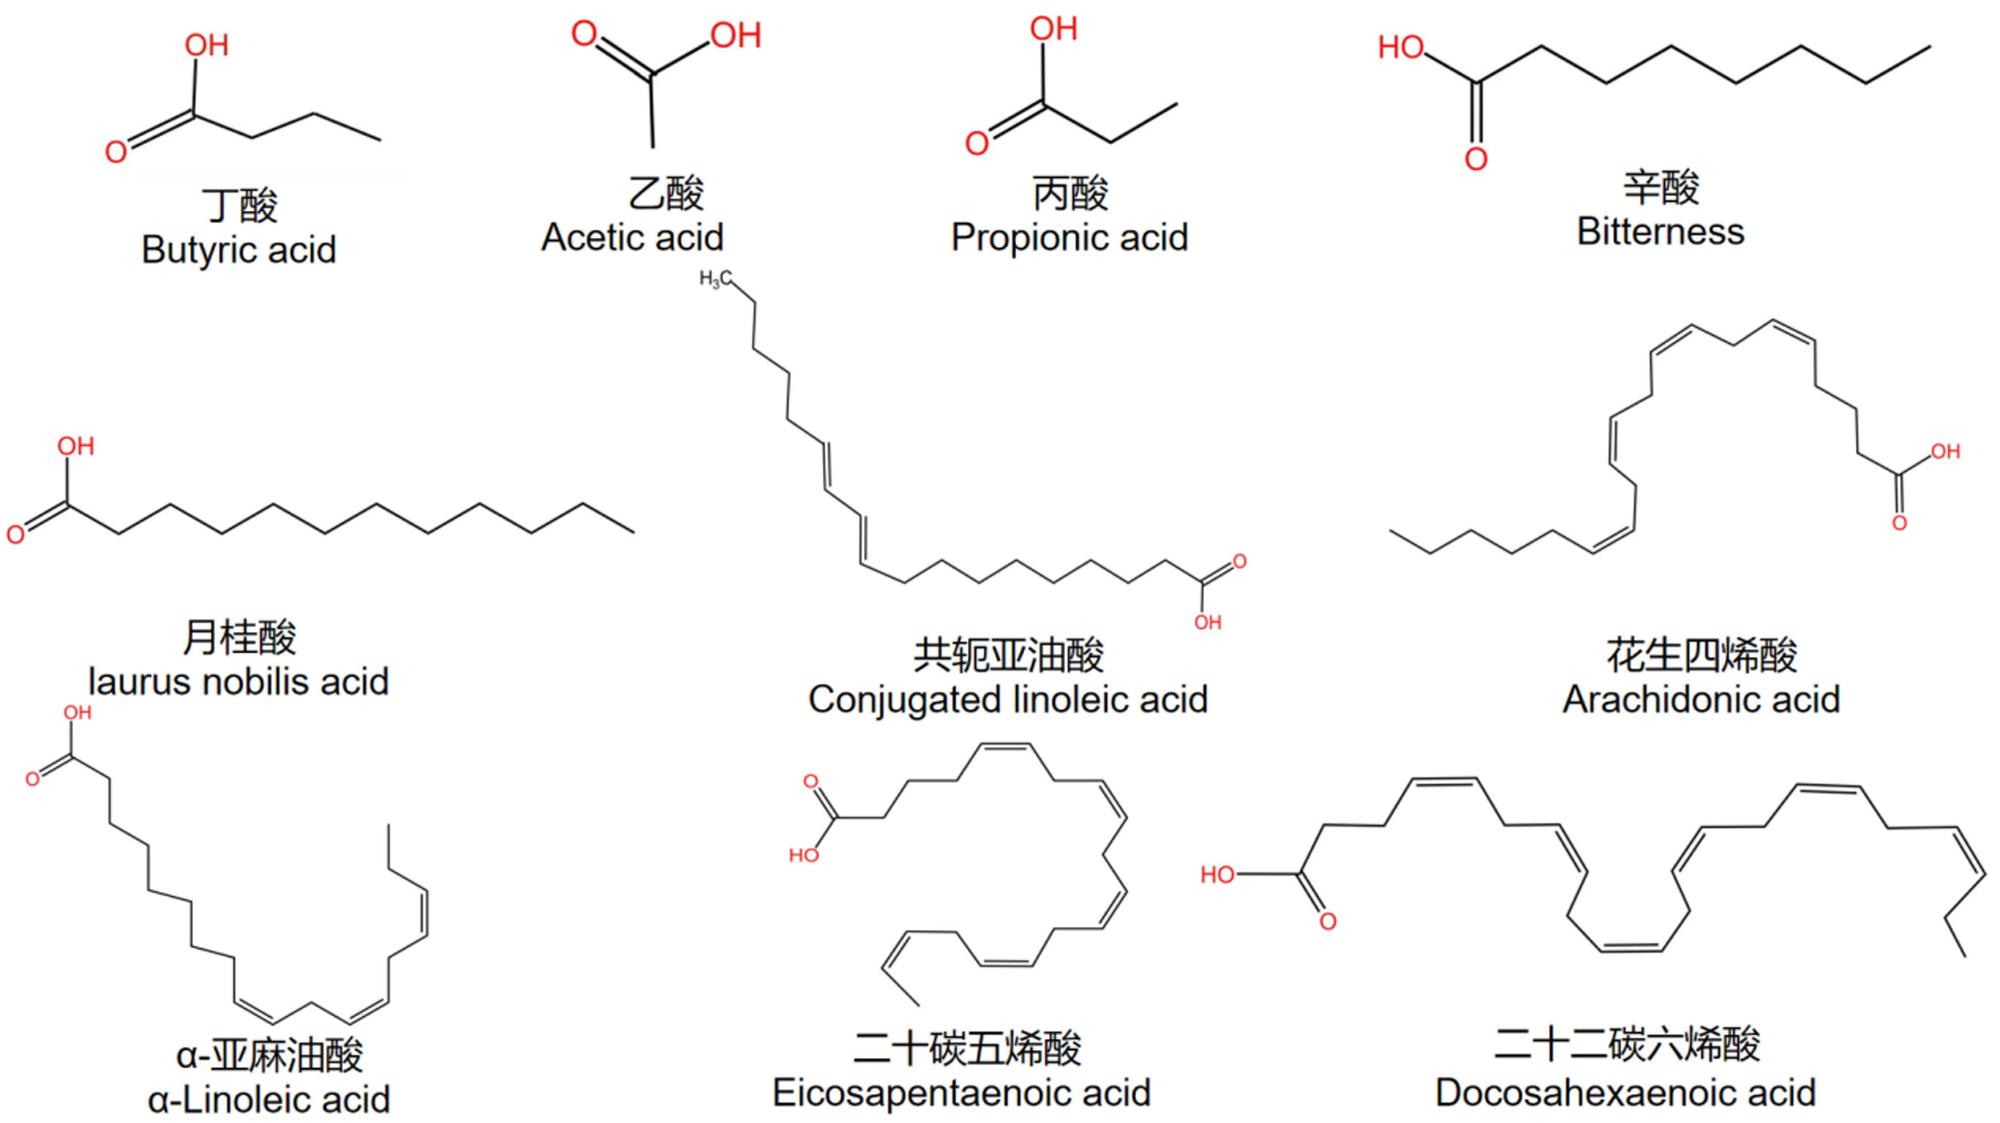
动物机体所需的脂肪酸来源主要通过肠道内微生物合成和采食获取。SCFA主要由肠道菌群发酵膳食纤维生成,而MCFA、PUFA则主要存在于天然油脂和深海鱼类中,需通过外源获取。SCFA常见的类型包括乙酸、丙酸、丁酸等,可以为肠道上皮细胞提供能量、维持肠道屏障功能。常见的MCFA包括月桂酸、辛酸等,具有快速供能、抗菌、抗病毒的作用。PUFA主要包括属于ω-3 PUFA的α-亚麻酸(α-linolenic acid,ALA)、二十二碳六烯酸(docosahexenoic acid,DHA)和二十碳五烯酸(eicosapentaenoic acid,EPA),其代谢物消退素、保护素具有抗炎作用并支持神经和胚胎等发育,ALA通过激活类固醇生成相关关键蛋白的表达,从而促进畜禽繁殖性能;而属于ω-6 PUFA的共轭亚油酸(conjugated linoleic acid,CLA)和花生四烯酸(arachidonic acid,AA)主要参与免疫调节过程,但摄入过量时可能引发炎症反应[3]。主要功能性脂肪酸的化学结构如图1所示。
图1 主要功能性脂肪酸的化学结构

Fig.1 Chemical structure of main functional fatty acids

1.2 功能性脂肪酸在体内的代谢

功能性脂肪酸的外源获取是通过饲料中的脂肪消化吸收完成的,而体内合成则主要在肝脏中进行。外源获取过程分为消化、吸收和转运3个阶段。首先,脂肪在小肠中被脂肪酶水解为游离脂肪酸和2-单酰甘油,其中PUFA的消化需要胆汁酸和脂肪酶共同作用,而SCFA和MCFA的消化无需胆汁酸作用。随后,游离脂肪酸通过自由扩散或依赖脂肪酸转运蛋白如脂肪酸转运蛋白、脂肪酸结合蛋白、小窝蛋白等进入肠细胞,在肠细胞内,脂肪酸与2-单酰甘油在滑面内质网重新合成甘油三酯,并与载脂蛋白A-I结合形成乳糜微粒,经载脂蛋白B48糖基化后,通过胞吐作用直接进入门静脉系统(而非淋巴系统)[4]。最后,乳糜微粒在肝脏内经过修饰,转化为极低密度脂蛋白(very low density lipoprotein,VLDL),并借助血液循环系统被运送至组织细胞,完成沉积过程[5]。肝脏是机体合成脂肪酸的主要场所,该过程以摄入的碳水化合物代谢产生的乙酰辅酶A为起始原料,通过特定的脂肪酸合成途径,最终生成脂肪酸[6]。合成的脂肪酸在肝脏内与甘油-3-磷酸结合生成甘油三酯,并通过VLDL分泌到血液中,最终沉积到脂肪组织或其他代谢需求的组织中。这一过程受到多种因素的调控,包括转录因子如固醇调节元件结合蛋白,激素如胰岛素、生长激素以及营养因素,以确保脂肪代谢保持动态平衡[7]

1.3 功能性脂肪酸对繁殖性能的调节作用

功能性脂肪酸对畜禽繁殖性能具有调节作用,主要体现在提升繁殖效率、提高后代质量及改善健康方面。研究报道,油酸通过增加小鼠卵巢颗粒细胞内脂滴中储存的甘油三酯水平并降低胆固醇酯水平,从而抑制类固醇的生成,减少卵泡囊和黄体的数量,从而降低小鼠生育能力[8]。月桂酸通过激活G蛋白偶联受体(G protein-coupled receptor,GPR)84、磷脂酰肌醇3-激酶(phosphatidylinositol 3-kinase,PI3K)和蛋白激酶B(protein kinase B,AKT)信号通路,促进青春期小鼠的乳腺发育[9]。研究发现,鞘磷脂通过调节蛋白激酶C-AKT-糖原合成酶激酶3β-细胞周期蛋白D3信号通路来调控子宫细胞增殖,其中鞘磷脂合成产生的二酰甘油和鞘氨醇-1-磷酸对蛋白激酶C和AKT信号通路的激活至关重要,大鼠子宫细胞增殖的同时其胞内鞘磷脂的合成也会增加[10]。AA能通过丝裂原活化蛋白激酶(adenosine monophosphate-activated protein kinase,MAPK)和PI3K/AKT信号通路中关键蛋白细胞外信号调节激酶1/2(extracellular signal-regulated kinase 1/2,ERK1/2)和AKT磷酸化调节牛卵泡颗粒细胞增殖、脂质积累和类固醇生成[11]。此外,ω-3 PUFA通过激活GPR120信号通路减轻炎症,并直接调节过氧化物酶体增殖物激活受体γ(peroxisome proliferator activated receptor γ,PPARγ)/CCAAT增强子结合蛋白α和趋化因子配体14-趋化因子受体4自分泌信号通路,诱导小鼠哺乳期乳腺脂肪生成和乳腺发育,进而改善乳腺功能[12]。Wang等[13]研究显示,三丁酸甘油酯也可通过增强卵巢抗氧化能力、抑制细胞凋亡及改善营养物质吸收的协同机制,保护卵巢功能,并提升肉种鸡繁殖性能。Zhao等[14]研究揭示,ALA通过激活c-Jun氨基末端激酶-类固醇生成因子1信号通路,上调睾酮合成调节关键蛋白、胆固醇侧链裂解酶、3β-羟基甾脱氢酶和类固醇17α-羟化酶/17,20裂解酶的表达,从而促进公鸡睾丸间质细胞中睾酮生物合成。这表明ALA通过调控特定类固醇生成酶的表达,进而促进睾酮的生物合成。此外,有研究指出,饲粮中添加富含亚油酸(linoleic acid,LA)和ALA的大豆油可促进小鼠睾丸激素的生成,这种膳食补充可激活黄体生成素-绒毛膜促性腺激素受体(luteinizing hormone chorionic gonadotropin receptor,LHCGR)信号通路,上调LHCGR、类固醇生成急性调节蛋白(steroids produce acute regulatory proteins,StAR)和细胞色素P450家族11亚家族A成员1(cytochrome P450 family 11 subfamily A member 1,CYP11A1)的表达,改善睾丸间质细胞中的类固醇合成功能,从而导致睾酮水平升高[15]。Sharma等[16]研究报道,ALA和CLA均可上调牛卵泡颗粒细胞脂肪酸转位酶转录表达,下调叉头盒L2、StAR、芳香酶、促卵泡激素受体、LHCGR的表达,并减少雌二醇(estradiol,E2)和孕酮(progesterone,P4)的生成,这可能会导致奶牛卵泡发育不良和卵巢周期性紊乱。功能性脂肪酸通过调控类固醇生成、卵泡发育、乳腺发育、睾酮合成及精子品质等相关信号通路,对畜禽繁殖性能发挥调节作用。功能性脂肪酸对畜禽繁殖性能的调控机制见表1
表1 功能性脂肪酸对畜禽繁殖性能的调控机制

Table 1 Regulatory mechanism of functional fatty acids on reproductive performance in livestock and poultry

生理过程
Physiological processes
关键脂肪酸
Key fatty acids
调控机制
Regulatory mechanism
参考文献
References
下丘脑-垂体-性腺轴调控
Regulation of hypothalamic-
pituitary-gonadal axis
PUFA 促进GnRH、FSH、LH和睾酮的分泌 黎琳琳等[17]
类固醇激素合成
Synthesis of steroid hormones
AA、LA 减少卵巢和子宫内膜中前列腺素F2α的
合成,维持黄体功能来间接支持促进P4合成
Mattos等[18]
颗粒细胞生长
Growth of granulocytes
AA 调节MAPK和PI3K/AKT信号通路中关键蛋白
ERK1/2和AKT磷酸化,促进颗粒细胞生长
Zhang等[11]
精子质量提升
Improvement of sperm quality
PUFA、CLA、
ALA、丁酸
增强配子膜流动性,增加精子密度、活力及
正常形态率,抑制细胞凋亡
Mohammadi等[19]
Liman等[20]、Qi等[21]
胚胎发育
Embryonic development
DHA、EPA 调控卵母细胞成熟、促进胎盘营养转运、
抗炎、免疫调节及支持神经发育
Politano等[22]
能量供应
Energy supply
棕榈酸 快速β-氧化为卵母细胞供能 Liu等[23]
糖脂代谢
Glycolipid metabolism
AA、LA、CLA、DHA 参与胰岛素分泌、葡萄糖吸收,调控脂
蛋白如VLDL的合成、分泌和代谢
Stein等[24]、李沙等[25]
夏珺等[26]、Wang等[27]

PUFA:多不饱和脂肪酸 polyunsaturated fatty acids;GnRH:促性腺激素释放激素 gonadotropin-releasing hormone;FSH:促卵泡激素 follicle-stimulating hormone;LH:促黄体素 lutropin;AA:花生四烯酸 arachidonic acid;LA:亚油酸 linoleic acid;P4:孕酮 progesterone;MAPK:丝裂原活化蛋白激酶 adenosine monophosphate-activated protein kinase;PI3K:磷脂酰肌醇3-激酶 phosphatidylinositol 3-kinase;AKT:蛋白激酶B protein kinase B;ERK1/2:细胞外信号调节激酶1/2 extracellular signal-regulated kinase 1/2;CLA:共轭亚油酸 conjugated linoleic acid;ALA:α-亚麻酸 α-linolenic acid;DHA:二十二碳六烯酸 docosahexenoic acid;EPA:二十碳五烯酸 eicosapentaenoic acid;VLDL:极低密度脂蛋白 very low density lipoprotein。

2 功能性脂肪酸通过微生物-肠-脑轴对繁殖性能的影响及作用机制

2.1 功能性脂肪酸对肠道菌群结构的调控作用

肠道微生物参与机体多种生理过程,对维持人和动物健康有着重要的作用。研究表明,功能性脂肪酸饮食能增加肠道有益菌的数量,并降低有害菌的数量,增强了宿主的肠道屏障,促进了营养物质的消化吸收[28]。肠道SCFA由结肠厌氧菌发酵膳食纤维和未消化碳水化合物生成,大部分在肠道消耗,少量乙酸和丙酸通过单羧酸转运蛋白被吸收入肝脏,作用于其他代谢途径。SCFA在动物肠道发挥强大的抗致病菌作用,酸性的肠道环境pH接近SCFA的酸度系数(pKa)值,使SCFA在酸性环境中以质子化形式自由扩散进入细菌细胞,进入后释放质子,导致细胞内pH下降[29]。SCFA能降低结肠pH,促进有益菌如乳杆菌属(Lactobacillus)和双歧杆菌属(Bifidobacterium)的繁殖[30]。此外,丁酸还为肠上皮细胞提供能量,同时结肠中丁酸和丙酸的摩尔比例也有所提升。研究表明,大鼠口服阿克曼菌属(Akkermansia)能显著增加SCFA产菌的数量[31]。嗜黏蛋白阿克曼菌(Akkermansia muciniphila)可保护小鼠免受辐射和化疗引起的肠道损伤,主要是由代谢生成的SCFA,通过激活GPR41/43信号通路和Wnt3/β-连环蛋白信号通路,实现双重作用:GPR41/43信号通路促进肠道干细胞增殖和上皮再生,Wnt3/β-连环蛋白信号通路激活维持肠干细胞自我更新能力,并确保受损上皮快速修复,同时增加黏液分泌,促进肠道益生菌增殖[32]。此外,SCFA和MCFA凭借其亲脂特性,以未解离的质子化形式穿透生物膜和细菌细胞壁,然后在细菌内部酸化细胞质,从而导致细菌死亡。SCFA和MCFA在pKa值上存在差异,MCFA能抑制细菌的信号传导过程并下调毒力基因表达,从而减少毒素的生成及降低其致病能力[33]。三丁酸甘油酯可促进母猪粪便拟杆菌门(Bacteroidetes)和螺旋体门(Spirochaetota)相对丰度上升,厚壁菌门(Firmicutes)相对丰度下降,促进SCFA生成菌的增殖,降低了肠道炎症的风险,缩短母猪分娩时间[34]。Garcia-So等[35]研究发现,ω-3 PUFA可以明显抑制怀孕小鼠胎盘炎症,减少具核梭杆菌(Fusobacterium nucleatum)在胎盘中的增殖,提高胚胎的存活率。0.2%的月桂酸单甘油脂可通过调节肠道菌群平衡、提高抗氧化能力和抗炎作用改善母猪的繁殖性能以及促进妊娠后期和哺乳期仔猪生长[36]。因此,功能性脂肪酸饮食可通过调节肠道菌群促进机体肠道健康,进而提升繁殖功能。

2.2 神经调节通路机制

作为宿主的重要组成部分,微生物-肠-脑轴参与机体免疫调节、神经交流等多项生理活动。功能性脂肪酸作为关键营养素,通过调节肠道微生物及代谢产物,经微生物-肠-脑轴神经调节通路影响畜禽繁殖性能的机制正逐渐被发掘。Miletta等[37]研究表明,丁酸通过激活GPR41/43促进细胞内钙离子(Ca2+)积累,增强垂体细胞中生长激素分泌。Eftekhar等[38]研究发现,生长激素可提高循环中胰岛素样生长因子-1水平,在促性腺激素协同下,刺激卵巢芳香化酶活性,增加颗粒细胞黄体生成素受体水平,加强促性腺激素作用,改善卵巢对促性腺激素敏感性。同时,生长激素脉冲分泌与性激素周期性变化相关,其脉冲幅度与E2水平呈正相关,与P4水平呈负相关。月桂酸则通过激活GPR84和PI3K/Akt信号通路来促进小鼠血清中胰岛素样生长因子-1和E2水平的增加,进而刺激乳腺发育[39]。Feng等[40]研究表示,丁酸纳通过肠道GPR41和多肽YY(polypeptide YY,PYY)组成启动肠道信号,这些信号通过肠-脑-卵巢轴,对下丘脑的激素水平产生调节作用,这种调节机制通过影响卵巢类固醇生成因子的表达,进而改善卵泡发育和颗粒细胞功能,降低黄体生成素和代谢紊乱,进而减少大鼠卵巢雄激素生成;同时调控卵巢类固醇代谢酶,恢复E2和P4水平,最终通过肠-脑-卵巢轴实现激素稳态。Lin等[41]研究显示,SCFA是肠道菌群中起主导作用的代谢产物,特别是丁酸经肠-脑轴进入系统循环、穿越血脑屏障到达大脑,刺激瘦素表达,激活下丘脑-垂体-性腺轴,促进雌性大鼠E2分泌及性腺发育。Andersen等[42]研究表明,MCFA的辛酸和癸酸促进星形胶质细胞谷氨酰胺合成,通过代谢耦合将谷氨酰胺转运至神经元,支持神经元中γ-氨基丁酸(γ-aminobutyric acid,GABA)合成。Watanabe等[43]研究发现,GABA在多数成熟的促性腺激素释放激素(gonadotropin-releasing hormone,GnRH)神经元中表现出异常兴奋,主要通过γ-氨基丁酸A型受体介导,引起膜去极化和钙离子内流,增加GnRH神经元放电活动和GnRH分泌。同时,也可以通过GABA和亲吻肽直接作用于GnRH神经元,或者GABA作用于亲吻肽神经元,以及亲吻肽作用于GABA神经元等方式调节GnRH分泌[44]。DHA和棕榈酸也可通过GPR120介导的下游PKC/MAPK和PI3K信号通路增加GnRH转录,表明DHA和棕榈酸可直接作用于GnRH神经元,调节性激素相关的基因表达[45]。功能性脂肪酸通过调节肠道微生物组成及代谢产物,经微生物-肠-脑轴神经调节通路影响畜禽繁殖性能。

2.3 神经内分泌调节通路机制

肠道菌群能够产生多种神经递质,如血清素、多巴胺、GABA,这些物质在调节性欲、生殖激素分泌和性行为方面起着至关重要的作用。SCFA通过与肠上皮细胞表达的游离脂肪酸受体2结合,引发肠内分泌细胞的钙信号反应,进而刺激迷走神经传入活动[46],而迷走神经连接肠道和大脑,将有关肠道状态的信息传递到中枢神经系统,从而影响内分泌系统的功能[47]。单不饱和及多不饱和磷脂酸可分别调节神经内分泌细胞的胞吐和融合孔的稳定性和扩张,从而改善机体健康[48]。研究发现,脂肪酸可以增加肠道Bifidobacterium相对丰度,Bifidobacterium通过调节肠道-大脑和下丘脑-垂体-卵巢轴,促进多囊性卵巢综合征小鼠神经内分泌平衡,并显著提高性激素水平,特别是促卵泡激素(follicle-stimulating hormone,FSH)和E2,具体作用机制可能通过改善肠道微生物群的多样性和组成,促进有益菌属如LactobacillusBifidobacterium的增殖,这些菌属与FSH、E2、白细胞介素-10(interleukin-10,IL-10)及脑源神经生长因子水平呈正相关,而与白细胞介素-6(interleukin-6,IL-6)、肿瘤坏死因子-α(tumor necrosis factor-α,TNF-α)、脂多糖(lipopolysaccharide,LPS)等炎症标志物水平呈负相关,通过降低炎症标志物水平并提升抗炎因子水平来调节炎症反应,进而促进激素水平的提升[49]
类似地,在大鼠中的研究显示,丁酸通过组蛋白H3第9位赖氨酸的乙酰化修饰(histone H3 lysine 9 acetylation,H3K9ac)表观调控激活PPARγ和过氧化物酶体增殖物激活受体-γ共激活因子-1α(peroxisome proliferator-activated receptor γ coactivator-1α,PGC-1α)信号通路,协同改善胆固醇代谢、线粒体功能及抗氧化能力,最终增强卵巢颗粒细胞的类固醇激素合成[50]。补充丁酸钠或通过饮食改变增加SCFA的水平也能提高公猪精子质量、精子活力和存活率[51],这些因素都受到下丘脑-垂体-卵巢轴的调控,SCFA可以通过刺激肠内分泌细胞释放肠道激素和肽类来间接调节肠-脑轴,还可以刺激胰高血糖素样肽-1、PYY和瘦素等激素的分泌[52-53],这些激素除了可以作用于大脑中的受体,还可以作用于迷走神经[54],进而可能影响机体生殖激素的分泌。也有研究发现,植物乳杆菌干预雌性大鼠后,大鼠肠道中产丁酸菌属显著富集,导致粪便丁酸水平升高,丁酸通过激活结肠上皮GPR41,上调其基因表达,进而刺激肠道PYY分泌,升高的PYY可能通过血脑屏障作用于下丘脑-垂体-性腺轴,抑制黄体生成素分泌并降低血清睾酮水平,最终改善卵巢形态异常和激素失衡[55]
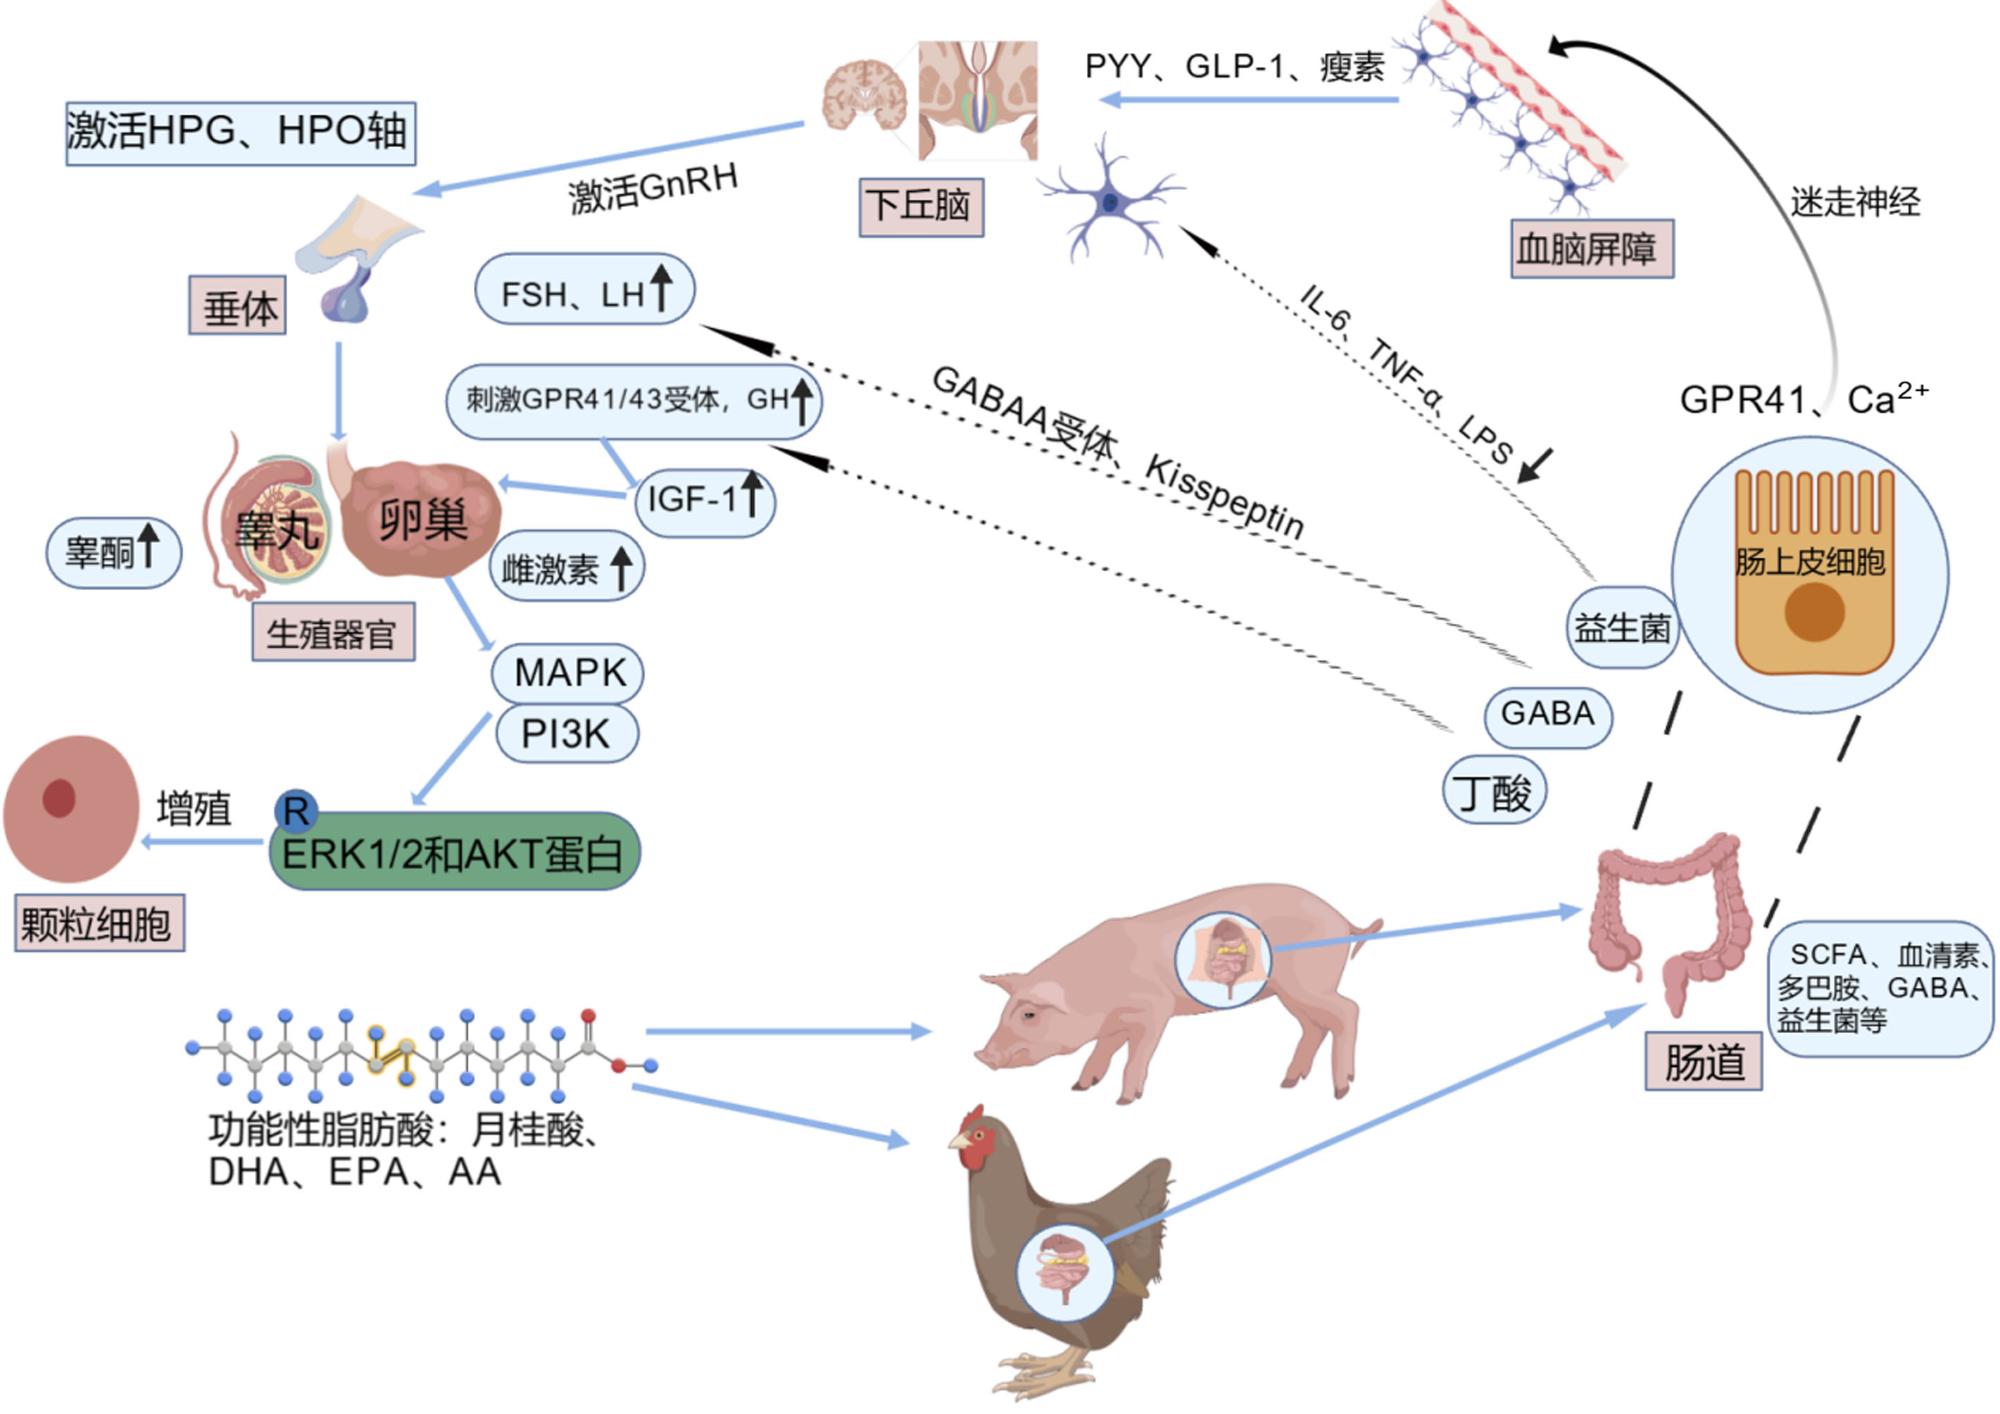
Zeng等[56]在母猪体内试验中表明,SCFA、MCFA联合使用共同激活PPARγ核受体,协同上调类固醇生成和子宫内膜容受性相关基因的表达,并特异性抑制肠道和阴道病原微生物,减少感染和炎症风险,维持妊娠早期稳定的激素和免疫环境。在母猪产后发情周期研究中,肠道菌群紊乱是导致母猪无法恢复发情的原因之一。研究发现,正常产后发情母猪中富集的益生菌群,如Lactobacillus和普雷沃菌属(Prevotella)能产生具有抗炎作用的SCFA,与FSH、E2、IL-10水平呈正相关[57],这可能也涉及脂肪酸通过调节肠-脑轴和下丘脑-垂体-卵巢轴来改善激素水平。有研究发现,丁酸盐通过组蛋白去乙酰化酶抑制活性重塑染色质结构,在色氨酸衍生芳香烃受体(aryl hydrocarbon receptor,AhR)激动剂存在时促进AhR向靶基因启动子的募集,从而增强AhR的激活效应[58],而AhR是一种配体依赖性转录因子,已有研究表明AhR信号通路在调控雌性生物体生殖方面发挥着重要作用,当AhR信号通路被激活后,会通过多种途径干扰生物体内源雌激素受体通路[59]。SCFA补充通过增加后备母猪肠道有益菌丰度及多样性、促进丙酸和丁酸等代谢物产生,经血液循环作用于卵巢,抑制颗粒细胞凋亡并促进卵泡发育[60]。同样地,ω-3 PUFA通过增加肠道有益菌相对丰度,抑制有害菌增殖,增加肠道菌群代谢产物,缓解肠道炎症,减少促炎因子进入血液循环,从而减轻神经炎症和血脑屏障破坏,同时在中枢神经系统中,EPA和DHA可通过减少皮质醇过度分泌抑制下丘脑-垂体-肾上腺轴过度激活,缓解神经应激损伤[61]。功能性脂肪酸通过调节肠道菌群及代谢产物经迷走神经、下丘脑-垂体-卵巢轴、下丘脑-垂体-性腺轴等通路影响生殖激素水平、类固醇生成及精子质量等,进而调控畜禽繁殖性能(图2)。
图2 功能性脂肪酸与微生物-肠-脑轴互作机制

HPG:下丘脑-垂体-性腺 hypothalamic-pituitary-gonadal;HPO:下丘脑-垂体-卵巢 hypothalamic-pituitary-ovarian;FSH:促卵泡素 follicle-stimulating hormone;LH:促黄体素 lutropin;GH:生长激素 growth hormone;IGF-1:胰岛素样生长因子1 insulin like growth factor-1;MAPK:丝裂原活化蛋白激酶 mitogen activated protein kinase;PI3K:磷脂酰肌醇3-激酶 phosphatidylinositol 3 kinase;AKT:蛋白激酶B protein kinase B;ERK1/2:细胞外信号调节激酶1/2 extracellular signal-regulated kinase 1/2;DHA:二十二碳六烯酸 docosahexenoic acid;EPA:二十碳五烯酸 eicosapentaenoic acid;AA:花生四烯酸 arachidonic acid;PYY:多肽YY polypeptide YY;GLP-1:胰高血糖素样肽-1 glucagon-like peptide-1;IL-6:白细胞介素-6 interleukin-6;TNF-α:肿瘤坏死因子-α tumor necrosis factor-α;LPS:脂多糖 lipopolysaccharide;GPR:G蛋白偶联受体 G protein-coupled receptor;Ca2+:钙离子 calcium ion;GABAA:γ-氨基丁酸A型受体 γ-amino butyric acid type A receptor;Kisspeptin:亲吻肽;GABA:γ-氨基丁酸 γ-aminobutyric acid;SCFA:短链脂肪酸 short-chain fatty acids。

Fig.2 Interaction mechanism between functional fatty acids and microbiota-gut-brain axis

3 功能性脂肪酸在畜禽繁殖中的应用

3.1 功能性脂肪酸在猪繁殖中的应用

种猪繁殖性能的高低对生猪养殖业有重要的决定性作用。Rosero等[62]研究报道,在母猪饲粮中补充ALA可使母猪迅速恢复发情,实现较高的妊娠率和较大的产仔数。杨建清[63]研究报道,在二元杂母猪妊娠后期饲粮中添加3.5%的椰子油可提高母猪采食量,并提高仔猪的初生重。在母猪妊娠期和泌乳期饲粮中分别添加15、30 g/kg富含ω-3长链脂肪酸(LCFA)的鱼油能提高妊娠期和哺乳期母猪血浆免疫球蛋白M(IgM)水平以及断奶仔猪血浆IL-6和白细胞介素-1β(interleukin-1β,IL-1β)水平,减少弱仔数[64]。Holen等[65]研究报道,哺乳母猪饲粮中添加LA和ALA可提高初乳和乳汁中LA和ALA含量,有助于提高仔猪生长和断奶重。在哺乳母猪饲养管理中,每日饲喂60 g富含ω-3 PUFA的鱼油能增加Lactobacillus和瘤胃球菌科UCG-014(Ruminococcaceae_UCG-014)相对丰度,促进E2和催乳素分泌[66]。长白公猪饲粮ω-3∶ω-6 PUFA比值由2.2升至约6.6,并协同添加高剂量维生素E,可通过富集DHA和强化抗氧化屏障来改善公猪精液品质[67]。因此,在种猪饲粮中添加不同功能性脂肪酸可提高母猪发情恢复、妊娠率、产仔数、初乳品质及仔猪质量,并改善公猪精液品质。

3.2 功能性脂肪酸在家禽繁殖中的应用

饲粮中添加不同类型的功能性脂肪酸对家禽的繁殖性能具有重要作用。饲粮中添加ω-3 PUFA可以改善罗氏种公鸡精液品质,提高种母鸡的产蛋率、种蛋受精率和孵化率[68]。Long等[69]研究报道,1%的亚麻酸可改善京粉蛋种公鸡精液中超氧化物歧化酶、谷胱甘肽过氧化物酶活性。Maina等[70]研究发现,富含DHA的藻油在不影响产蛋量、采食量及蛋重等前提下,显著增加了鸡蛋蛋壳厚度,并大幅提高鸡蛋中DHA含量,同时降低ω-3∶ω-6 PUFA比值至健康理想范围。研究显示,在饲粮中添加富含ω-3 PUFA的鱼油,可改善精子质量,提高ω-3 PUFA比例,并降低ω-3∶ω-6 PUFA比值,主要是ω-3 PUFA通过饮食调节改变脂肪酸谱,并增加精子磷脂双层中ω-3 PUFA比例,进而提升公鸡的精液质量、生殖激素水平和精子脂肪酸组成[71]。此外,有研究提出,在含CLA饲粮中添加适量大豆油可调整白羽肉种鸡种蛋脂肪酸组成,并增强其抗氧化能力,从而在一定程度上恢复受精蛋的孵化率[72]。Thanabalan等[73]研究表明,饲粮中添加DHA和ALA可促进罗氏708肉种鸡母源抗体转移、B细胞增殖和成熟,增加种蛋免疫球蛋白A水平,从而改善子代肉鸡生长性能。因此,饲粮中添加不同类型的功能性脂肪酸可提高种公鸡精液品质和种母鸡繁殖性能。

3.3 功能性脂肪酸在反刍动物繁殖中的应用

功能性脂肪酸在反刍动物中需通过过瘤胃保护技术规避瘤胃微生物的降解,才能发挥其生物作用。张平等[74]研究发现,饲粮中添加2%~3%的棕榈脂肪粉显著提高了奶牛的产奶量、4%标准乳产量以及乳脂率,同时改善了饲料效率和养分消化率,并促进了瘤胃发酵。许鹏等[75]研究发现,饲粮中添加200 g/d的过瘤胃脂肪酸显著提高了奶牛牛奶中的乳蛋白率,降低了血清丙二醛含量,改善了体况评分,同时添加过瘤胃不饱和脂肪还提升了牛奶中油酸和LA含量,从而改善了乳品质。Hanno等[76]向泌乳奶牛的饲粮中添加了1.5%的高油酸大豆油,显著提高了牛奶中的乳脂浓度,增加了表观全消化道脂肪消化率,并增加了背脂厚度。De Souza等[77]研究发现,改变饲粮棕榈酸和油酸的比例(约80%棕榈酸和10%油酸),在奶牛产后即刻和结转期显著增加了干物质摄入量、牛奶产量、能量校正乳以及乳脂产量,同时减少了体重和体况评分的损失。补充PUFA可促进卵泡发育,随ω-3 PUFA补充量增加,母羊血浆和卵泡液中消退素水平及谷胱甘肽过氧化物酶和GPR32的表达水平呈线性增加,而IL-1β和环氧化酶-2的表达水平呈线性降低[78]。功能性脂肪酸需通过过瘤胃保护技术在反刍动物中发挥作用,可提高繁殖性能,改善乳品质量,发挥抗炎、抗氧化等作用。

4 小结与展望

畜禽通过内源合成和外源摄取获得功能性脂肪酸,不仅可以为机体提供能量,还对畜禽的繁殖性能有一定调节作用。目前,研究多关注脂肪酸对类固醇激素合成的影响,而通过微生物-肠-脑轴对FSH和LH调节以及卵泡发育和黄体功能维持中的多方面作用研究报道较少。因此,未来关于功能性脂肪酸对繁殖性能的研究可重点围绕微生物-肠-脑轴这一关键信号通路展开,建立特定生理阶段的理想脂肪酸平衡模式,并通过整合多组学数据,借助人工智能技术解析复杂网络调控通路,明确功能性脂肪酸对畜禽的调控机制。同时,在精准营养体系下,开发智能饲喂方案,实现功能性脂肪酸的最佳配比与高效利用,从而全面提升畜禽繁殖潜能。
[1]
CHEN Y X, TOUBOUL R, CHEN Y, et al. Strategic delivery of omega-3 fatty acids for modulating inflammatory neurodegenerative diseases[J]. Frontiers in Aging Neuroscience, 2025, 17:1535094.

DOI

[2]
SUNDARAM T S, GIROMINI C, REBUCCI R, et al. Role of omega-3 polyunsaturated fatty acids,citrus pectin,and milk-derived exosomes on intestinal barrier integrity and immunity in animals[J]. Journal of Animal Science and Biotechnology, 2022, 13(1):40.

DOI

[3]
RUTTING S, PAPANICOLAOU M, XENAKI D, et al. Dietary ω-6 polyunsaturated fatty acid arachidonic acid increases inflammation,but inhibits ECM protein expression in COPD[J]. Respiratory Research, 2018, 19(1):211.

DOI

[4]
黄海, 米杨, 田苗苗, 等. 膳食脂肪的餐后代谢与脂蛋白脂肪酶研究进展[J]. 食品科学, 2015, 36(9):235-241.

DOI

HUANG H, MI Y, TIAN M M, et al. Metabolism of postprandial dietary fat and lipoprotein lipase[J]. Food Science, 2015, 36(9):235-241. (in Chinese)

DOI

[5]
陈伟, 林映才, 张罕星, 等. 家禽脂肪酸代谢及其在禽蛋中的沉积和营养调控[J]. 动物营养学报, 2012, 24(2):204-211.

CHEN W, LIN Y C, ZHANG H X, et al. Fatty acids:metabolism in poultry and deposition and nutritional regulation in eggs[J]. Chinese Journal of Animal Nutrition, 2012, 24(2):204-211. (in Chinese)

[6]
SCHÖNFELD P, WOJTCZAK L. Short- and medium-chain fatty acids in energy metabolism:the cellular perspective[J]. Journal of Lipid Research, 2016, 57(6):943-954.

DOI

[7]
秦昆鹏, 李响, 尹月, 等. 鸡的脂肪生成及其调控机制[J]. 动物营养学报, 2022, 34(11):6860-6872.

DOI

QIN K P, LI X, YIN Y, et al. Adipogenesis in chicken and its regulation mechanism[J]. Chinese Journal of Animal Nutrition, 2022, 34(11):6860-6872. (in Chinese)

DOI

[8]
ZHOU X G, MO Z Y, LI Y K, et al. Oleic acid reduces steroidogenesis by changing the lipid type stored in lipid droplets of ovarian granulosa cells[J]. Journal of Animal Science and Biotechnology, 2022, 13(1):27.

DOI PMID

[9]
MENG Y Y, ZHANG J, ZHANG F L, et al. Lauric acid stimulates mammary gland development of pubertal mice through activation of GPR84 and PI3K/Akt signaling pathway[J]. Journal of Agricultural and Food Chemistry, 2017, 65(1):95-103.

DOI PMID

[10]
CERBÓN J, BARANDA-AVILA N, FALCÓN-MUÑOZ A, et al. Sphingolipid synthesis and role in uterine epithelia proliferation[J]. Reproduction, 2018, 156(2):173-183.

DOI

[11]
ZHANG N N, WANG L Q, LUO G Y, et al. Arachidonic acid regulation of intracellular signaling pathways and target gene expression in bovine ovarian granulosa cells[J]. Animals, 2019, 9(6):374.

DOI

[12]
LI B F, SU S L, YUAN S Y, et al. Omega-3 fatty acids regulate mammary gland lipogenesis and development via Gαs-mediated cAMP-EPAC signaling pathway[J]. Research, 2025, 8:0767.

DOI

[13]
WANG J P, ZHANG H Y, BAI S P, et al. Dietary tributyrin improves reproductive performance,antioxidant capacity,and ovary function of broiler breeders[J]. Poultry Science, 2021, 100(11):101429.

DOI

[14]
ZHAO Z X, SHANG M Y, LONG C, et al. α-linolenic acid-regulated testosterone biosynthesis via activation of the JNK-SF-1 signaling pathway in primary rooster Leydig cells[J]. Theriogenology, 2023, 209:170-177.

DOI

[15]
苏雨. 大豆油和花生四烯酸油摄入增加对睾丸间质细胞睾酮合成的影响[D]. 硕士学位论文. 济南: 山东大学, 2021.

SU Y. Effects of increasing intake of soybean oil and arachidonic acid oil on synthesis of testosterone in Leydig cells[D]. Master’s Thesis. Ji’nan: Shandong University, 2021. (in Chinese)

[16]
SHARMA A, BADDELA V S, ROETTGEN V, et al. Effects of dietary fatty acids on bovine oocyte competence and granulosa cells[J]. Frontiers in Endocrinology, 2020, 11:87.

DOI PMID

[17]
黎琳琳, 胡韶华, 尹小琴, 等. 特发性中枢性性早熟女童血清不饱和游离脂肪酸谱的变化及其与体质量指数、性激素水平的相关性分析[J]. 上海交通大学学报(医学版), 2021, 41(11):1405-1411.

LI L L, HU S H, YIN X Q, et al. Changes of serum unsaturated free fatty acid profiles in girls with idiopathic central precocious puberty and their correlations with body mass index and sex hormones[J]. Journal of Shanghai Jiaotong University (Medical Science), 2021, 41(11):1405-1411. (in Chinese)

[18]
MATTOS R, STAPLES C R, THATCHER W W. Effects of dietary fatty acids on reproduction in ruminants[J]. Reviews of Reproduction, 2000, 5(1):38-45.

PMID

[19]
MOHAMMADI H, GOLBABAEI F, DEHGHAN S F, et al. The influence of vitamin E and omega-3 fatty acids on reproductive health indices among male workers exposed to electromagnetic fields[J]. American Journal of Men’s Health, 2022, 16(1):15579883221074821.

[20]
LIMAN M S, FRANCO V, CARDOSO C L, et al. Effects of dietary supplementation of conjugated linoleic acids and their inclusion in semen extenders on bovine sperm quality[J]. Animals, 2021, 11(2):483.

DOI

[21]
QI J J, SUN Y, CHEN Z Q, et al. Sodium butyrate promotes synthesis of testosterone and meiosis of hyperuricemic male mice[J]. Scientific Reports, 2025, 15(1):14757.

DOI

[22]
POLITANO C A, LÓPEZ-BERROA J. Omega-3 fatty acids and fecundation,pregnancy and breastfeeding[J]. Revista Brasileira de Ginecologia e Obstetricia, 2020, 42(3):160-164.

DOI

[23]
LIU T, QU J X, TIAN M Y, et al. Lipid metabolic process involved in oocyte maturation during folliculogenesis[J]. Frontiers in Cell and Developmental Biology, 2022, 10:806890.

DOI

[24]
STEIN D T, STEVENSON B E, CHESTER M W, et al. The insulinotropic potency of fatty acids is influenced profoundly by their chain length and degree of saturation[J]. Journal of Clinical Investigation, 1997, 100(2):398-403.

PMID

[25]
李沙, 苏文, 张晓燕, 等. 花生四烯酸代谢与肝脏糖脂代谢稳态调控[J]. 生理学报, 2021, 73(4):657-664.

LI S, SU W, ZHANG X Y, et al. Arachidonic acid metabolism in liver glucose and lipid homeostasis[J]. Acta Physiologica Sinica, 2021, 73(4):657-664. (in Chinese)

[26]
夏珺, 郑明月, 李灵杰, 等. 共轭亚油酸改善肥胖糖尿病小鼠的糖脂代谢[J]. 南方医科大学学报, 2019, 39(6):740-746.

XIA J, ZHENG M Y, LI L J, et al. Conjugated linoleic acid improves glucose and lipid metabolism in diabetic mice[J]. Journal of Southern Medical University, 2019, 39(6):740-746. (in Chinese)

[27]
WANG Y, LIN Q W, ZHENG P P, et al. Effects of eicosapentaenoic acid and docosahexaenoic acid on chylomicron and VLDL synthesis and secretion in Caco-2 cells[J]. BioMed Research International, 2014, 2014:684325.

[28]
曹战江, 于健春, 康维明, 等. 补充n-3多不饱和脂肪酸对高脂饮食大鼠肠道菌群及门静脉血内毒素的影响[J]. 中国医学科学院学报, 2014, 36(5):496-500.

DOI

CAO Z J, YU J C, KANG W M, et al. Effect of n-3 polyunsaturated fatty acids on gut microbiota and endotoxin levels in portal vein of rats fed with high-fat diet[J]. Acta Academiae Medicinae Sinicae, 2014, 36(5):496-500. (in Chinese)

[29]
LING C, REN L L, SONG Y R, et al. Intestinal short-chain fatty acids spatially regulate the antibiotic tolerance and virulence of avian pathogenic Escherichia coli[J]. Poultry Science, 2025, 104(4):104917.

DOI

[30]
AKHTAR M, CHEN Y, MA Z Y, et al. Gut microbiota-derived short chain fatty acids are potential mediators in gut inflammation[J]. Animal Nutrition, 2022, 8:350-360.

DOI PMID

[31]
YAN J L, PAN Y B, SHAO W M, et al. Beneficial effect of the short-chain fatty acid propionate on vascular calcification through intestinal microbiota remodelling[J]. Microbiome, 2022, 10(1):195.

DOI PMID

[32]
KIM S, SHIN Y C, KIM T Y, et al. Mucin degrader Akkermansia muciniphila accelerates intestinal stem cell-mediated epithelial development[J]. Gut Microbes, 2021, 13(1):1892441.

DOI

[33]
SZABÓ R T, KOVÁCS-WEBER M, ZIMBORÁN Á, et al. Effects of short- and medium-chain fatty acids on production,meat quality,and microbial attributes-a review[J]. Molecules, 2023, 28(13):4956.

DOI

[34]
LIN Y, LI D, MA Z, et al. Maternal tributyrin supplementation in late pregnancy and lactation improves offspring immunity,gut microbiota,and diarrhea rate in a sow model[J]. Frontiers in Microbiology, 2023, 14:1142174.

DOI

[35]
GARCIA-SO J, ZHANG X W, YANG X H, et al. Omega-3 fatty acids suppress fusobacterium nucleatum-induced placental inflammation originating from maternal endothelial cells[J]. JCI Insight, 2019, 4(3):e125436.

DOI

[36]
LI D, YANG M, MA Z, et al. Glycerol monolaurate complex improved antioxidant,anti-inflammation,and gut microbiota composition of offspring in a sow-piglet model[J]. Veterinary Sciences, 2025, 12(1):24.

DOI

[37]
MILETTA M C, PETKOVIC V, EBLÉ A, et al. Butyrate increases intracellular calcium levels and enhances growth hormone release from rat anterior pituitary cells via the G-protein-coupled receptors GPR41 and 43[J]. PLoS One, 2014, 9(10):e107388.

DOI

[38]
EFTEKHAR M, AFLATOONIAN A, MOHAMMADIAN F, et al. Adjuvant growth hormone therapy in antagonist protocol in poor responders undergoing assisted reproductive technology[J]. Archives of Gynecology and Obstetrics, 2013, 287(5):1017-1021.

DOI PMID

[39]
LANG L, LIANG S, ZHANG F, et al. Knockdown of the VEGFB/VEGFR1 signaling suppresses pubertal mammary gland development of mice via the inhibition of PI3K/Akt pathway[J]. International Journal of Biological Macromolecules, 2024; 264(Pt.2):130782.

[40]
FENG X P, XIAO J, WANG D C, et al. Butyric acid ameliorates PCOS-related reproductive dysfunction through gut-brain-ovary axis signaling and ovarian steroidogenic factor activation[J]. Frontiers in Endocrinology, 2025, 16:1604302.

DOI

[41]
LIN C Y, NGUYEN N N, TSAI W L, et al. Aspartame intake delayed puberty onset in female offspring rats and girls[J]. Molecular Nutrition & Food Research, 2024, 68(5):2300270.

[42]
ANDERSEN J V, WESTI E W, JAKOBSEN E, et al. Astrocyte metabolism of the medium-chain fatty acids octanoic acid and decanoic acid promotes GABA synthesis in neurons via elevated glutamine supply[J]. Molecular Brain, 2021, 14(1):132.

DOI PMID

[43]
WATANABE M, FUKUDA A, NABEKURA J. The role of GABA in the regulation of GnRH neurons[J]. Frontiers in Neuroscience, 2014, 8:387.

DOI PMID

[44]
DI GIORGIO N P, BIZZOZZERO-HIRIART M, LIBERTUN C, et al. Unraveling the connection between GABA and kisspeptin in the control of reproduction[J]. Reproduction, 2019, 157(6):R225-R233.

[45]
TRAN D Q, RAMOS E H, BELSHAM D D. Induction of Gnrh mRNA expression by the ω-3 polyunsaturated fatty acid docosahexaenoic acid and the saturated fatty acid palmitate in a GnRH-synthesizing neuronal cell model,mHypoA-GnRH/GFP[J]. Molecular and Cellular Endocrinology, 2016, 426:125-135.

DOI

[46]
WANG X Z, ZHANG P, ZHANG X. Probiotics regulate gut microbiota:an effective method to improve immunity[J]. Molecules, 2021, 26(19):6076.

DOI

[47]
BREIT S, KUPFERBERG A, ROGLER G, et al. Vagus nerve as modulator of the brain-gut axis in psychiatric and inflammatory disorders[J]. Frontiers in Psychiatry, 2018, 9:44.

DOI PMID

[48]
TANGUY E, COSTÉ DE BAGNEAUX P, KASSAS N, et al. Mono- and poly-unsaturated phosphatidic acid regulate distinct steps of regulated exocytosis in neuroendocrine cells[J]. Cell Reports, 2020, 32(7):108026.

DOI

[49]
DONG Y, YANG S N, ZHANG S, et al. Modulatory impact of Bifidobacterium longum subsp.longum BL 21 on the gut-brain-ovary axis in polycystic ovary syndrome:insights into metabolic regulation,inflammation mitigation,and neuroprotection[J]. mSphere, 2025, 10(2):e0088724.

DOI

[50]
YE Q H, ZENG X F, WANG S, et al. Butyrate drives the acetylation of histone H3K9 to activate steroidogenesis through PPARγ and PGC1α pathways in ovarian granulosa cells[J]. The FASEB Journal, 2021, 35(2):e21316.

DOI

[51]
LIN Y, WANG K, CHE L Q, et al. The improvement of semen quality by dietary fiber intake is positively related with gut microbiota and SCFA in a boar model[J]. Frontiers in Microbiology, 2022, 13:863315.

DOI

[52]
NØHR M K, PEDERSEN M H, GILLE A, et al. GPR41/FFAR3 and GPR43/FFAR2 as cosensors for short-chain fatty acids in enteroendocrine cells vs FFAR3 in enteric neurons and FFAR2 in enteric leukocytes[J]. Endocrinology, 2013, 154(10):3552-3564.

DOI PMID

[53]
TOLHURST G, HEFFRON H, LAM Y S, et al. Short-chain fatty acids stimulate glucagon-like peptide-1 secretion via the G-protein-coupled receptor FFAR2[J]. Diabetes, 2012, 61(2):364-371.

DOI PMID

[54]
ABBOTT C R, MONTEIRO M, SMALL C J, et al. The inhibitory effects of peripheral administration of peptide YY(3-36) and glucagon-like peptide-1 on food intake are attenuated by ablation of the vagal-brainstem-hypothalamic pathway[J]. Brain Research, 2005, 1044(1):127-131.

PMID

[55]
HE Y F, MEI L Y, WANG L Y, et al. Lactiplantibacillus plantarum CCFM1019 attenuate polycystic ovary syndrome through butyrate dependent gut-brain mechanism[J]. Food & Function, 2022, 13(3):1380-1392.

[56]
ZENG X Z, LI S Y, YE Q H, et al. The combined use of medium- and short-chain fatty acids improves the pregnancy outcomes of sows by enhancing ovarian steroidogenesis and endometrial receptivity[J]. Nutrients, 2022, 14(20):4405.

DOI

[57]
LIU M, ZHANG J, ZHOU Y Y, et al. Gut microbiota affects the estrus return of sows by regulating the metabolism of sex steroid hormones[J]. Journal of Animal Science and Biotechnology, 2023, 14(1):155.

DOI PMID

[58]
MODOUX M, ROLHION N, LEFEVRE J H, et al. Butyrate acts through HDAC inhibition to enhance aryl hydrocarbon receptor activation by gut microbiota-derived ligands[J]. Gut Microbes, 2022, 14(1):2105637.

DOI

[59]
谢昕岑, 于淼, 汝少国. 基于AhR信号通路的抗雌激素效应及其机制研究进展[J]. 生态毒理学报, 2021, 16(5):148-159.

XIE X C, YU M, RU S G. Research advances of anti-estrogenic effect based on AhR signaling pathway and its mechanism[J]. Asian Journal of Ecotoxicology, 2021, 16(5):148-159. (in Chinese)

[60]
XU B Y, QIN W X, CHEN Y W, et al. Dietary short-chain fatty acids supplementation improves reproductive performance and gut microbiota in gilts[J]. The Journal of Nutrition, 2025, 155(4):1089-1098.

DOI

[61]
ZINKOW A, GRODZICKI W, CZERWIÑSKA M, et al. Molecular mechanisms linking omega-3 fatty acids and the gut-brain axis[J]. Molecules, 2024, 30(1):71.

DOI

[62]
ROSERO D S, BOYD R D, ODLE J, et al. Optimizing dietary lipid use to improve essential fatty acid status and reproductive performance of the modern lactating sow:a review[J]. Journal of Animal Science and Biotechnology, 2016, 7(1):34.

DOI

[63]
杨建清. 不同类型油脂对母猪繁殖性能及血清生化指标的影响[J]. 畜牧兽医科学, 2020(19):55-56.

YANG J Q. Effect of different types of oils and fats on reproductive performance and serum biochemical parameters of sows[J]. Graziery Veterinary Sciences (Electronic Version), 2020(19):55-56. (in Chinese)

[64]
LLAURADÓ-CALERO E, BADIOLA I, SAMARRA I, et al. Eicosapentaenoic acid- and docosahexaenoic acid-rich fish oil in sow and piglet diets modifies blood oxylipins and immune indicators in both,sows and suckling piglets[J]. Animal, 2022, 16(10):100634.

DOI

[65]
HOLEN J P, WOODWORTH J C, TOKACH M D, et al. Evaluation of essential fatty acids in lactating sow diets on sow reproductive performance,colostrum and milk composition,and piglet survivability[J]. Journal of Animal Science, 2022, 100(6):skac167.

[66]
GE Z H, AN Y L, LAN W, et al. Effects of dietary supplementation of omega-3 PUFA enriched fish oil during late-pregnancy and lactation on reproductive performance,immune activity and fecal microbiota composition in postpartum sows[J]. Veterinary Sciences, 2025, 12(2):139.

DOI

[67]
LIU Q, ZHOU Y F, DUAN R J, et al. Effects of dietary n-6∶n-3 fatty acid ratio and vitamin E on semen quality,fatty acid composition and antioxidant status in boars[J]. Animal Reproduction Science, 2015, 162:11-19.

DOI

[68]
SAFARI ASL R, SHARIATMADARI F, SHARAFI M, et al. Improvements in semen quality,sperm fatty acids,and reproductive performance in aged ross breeder roosters fed a diet supplemented with a moderate ratio of n-3:n-6 fatty acids[J]. Poultry Science, 2018, 97(11):4113-4121.

DOI

[69]
LONG C, YIN X F, SHENG X H, et al. Dietary alpha-linolenic acid supplementation enhances semen quality,antioxidant capacity,and sperm survival in aging breeder roosters[J]. Poultry Science, 2024, 103(12):104252.

DOI

[70]
MAINA A N, LEWIS E, KIARIE E G. Egg production, egg quality,and fatty acids profiles in eggs and tissues in Lohmann LSL lite hens fed algal oils rich in docosahexaenoic acid (DHA)[J]. Poultry Science, 2023, 102(10):102921.

DOI

[71]
TEYMOURI ZADEH Z, SHARIATMADARI F, SHARAFI M, et al. Amelioration effects of n-3,n-6 sources of fatty acids and rosemary leaves powder on the semen parameters,reproductive hormones,and fatty acid analysis of sperm in aged ross broiler breeder roosters[J]. Poultry Science, 2020, 99(2):708-718.

DOI

[72]
刘雪兰, 张燕, 伏春燕, 等. 肉种鸡共轭亚油酸(CLA)饲粮中添加不同比例的大豆油对其繁殖性能的影响[J]. 安徽农业科学, 2018, 46(19):96-99.

LIU X L, ZHANG Y, FU C Y, et al. Effects of conjugated linoleic acid diets supplemented with different proportions of soybean oil on reproductive performance of chicken breeders[J]. Journal of Anhui Agricultural Sciences, 2018, 46(19):96-99. (in Chinese)

[73]
THANABALAN A, DREGER R, KIARIE E G. Significance of successive feeding of sources of n-3 fatty acids to broiler breeders and their progeny on growth performance,intestinal lesion scores,lymphoid organs weight and plasma immunoglobulin A in broiler chickens challenged with Eimeria[J]. Poultry Science, 2024, 103(7):103796.

DOI

[74]
张平, 郭刚, 霍文婕, 等. 日粮添加棕榈脂肪粉对泌乳牛产奶性能、养分消化率和瘤胃发酵的影响[J]. 中国畜牧杂志, 2020, 56(2):136-140.

ZHANG P, GUO G, HUO W J, et al. Effects of dietary palm fat powder on milking performance,nutrient digestibility and rumen fermentation in lactating cows[J]. Chinese Journal of Animal Science, 2020, 56(2):136-140. (in Chinese)

[75]
许鹏, 杨致玲, 吴树峰, 等. 饲粮添加不同过瘤胃脂肪源对奶牛生产性能及牛奶中脂肪酸组成的影响[J]. 动物营养学报, 2021, 33(5):2727-2737.

DOI

XU P, YANG Z L, WU S F, et al. Effects of dietary different rumen protected fat sources on performance and milk fatty acid composition of dairy cattle[J]. Chinese Journal of Animal Nutrition, 2021, 33(5):2727-2737. (in Chinese)

[76]
HANNO S L, HURST A M, WEAVER K, et al. High oleic soybean oil maintains milk fat and increases apparent total-tract fat digestibility and fat deposition in lactating dairy cows[J]. JDS Communications, 2024, 5(4):287-292.

DOI PMID

[77]
DE SOUZA J, PROM C M, LOCK A L. Altering the ratio of dietary palmitic and oleic acids affects production responses during the immediate postpartum and carryover periods in dairy cows[J]. Journal of Dairy Science, 2021, 104(3):2896-2909.

DOI PMID

[78]
CARRANZA-MARTIN A C, GARCIA-GUERRA A, RELLING A E. Effects of polyunsaturated fatty acid supplementation on plasma and follicular fluid resolvin D1 concentration and mRNA abundance in granulosa cells in ewes[J]. Journal of Animal Science, 2023, 101:skad310.

文章导航

/