RESEARCH PAPER

Effects of Compound Plant Nutrients on Rumen Fermentation Parameters, Rumen Microbiota and Fatty Acid Composition of Longissimus dorsi Muscle in Finishing Small Tail Han Sheep

  • WANG Yuan , 1, 2, 3 ,
  • WANG Wenwen 1, 2 ,
  • YANG Yi 1, 2 ,
  • GAO Chang 1, 2 ,
  • GUO Tao 1, 2 ,
  • DUAN Ting 1, 2 ,
  • LIU Na 1, 2 ,
  • AN Xiaoping 1, 2 ,
  • QI Jingwei , 1, 2, *
Expand
  • 1 College of Animal Science, Inner Mongolia Agricultural University, Hohhot 010018, China
  • 2 Inner Mongolia Herbivorous Livestock Feed Engineering and Technology Research Center, Hohhot 010018, China
  • 3 Anhui Province Key Laboratory of Animal Nutrition Regulation and Health, Anhui University of Science and Technology, Chuzhou 233100, China
* professor, E-mail:

Received date: 2022-05-25

  Online published: 2023-01-11

Abstract

This study was conducted to investigate the effects of compound plant nutrients (CPN) on rumen fermentation parameters, rumen microbiota and fatty acid composition of longissimus dorsi muscle in finishing small tail Han sheep. Sixteen 4-month-old finishing small tail Han sheep with an initial body weight (BW) of (24.18±0.31) kg were randomly divided into two groups, namely, with 8 replicates per group and 1 sheep per replicate. The sheep in the control group were fed a basal diet, whereas the sheep of the control group (CPN group) was fed the basal diet supplementation with 3 ‰ CPN. The experiment lasted for 97 days after 7 days adaption. The results showed as follows: compared with the control group, 1) adding CPN decreased the concentration of ammonia nitrogen (NH3-N) (P<0.05); 2) CPN supplementation affected beta diversity of rumen microbiota; 3) the relative abundance of Acidobacteriota, Erysipelotrichaceae_UCG-002, Lactobacillus, and Megasphaera were enhanced by adding CPN (P<0.05), whereas, the relative abundance of Bacteroidetes and Prevotella was lower (P<0.05); 4) the supplementation of CPN had no significant effect on fatty acid composition of longissimus dorsi muscle of fattening small-tailed Han sheep (P>0.05); 5) the contents of total MUFA, C18∶1n9c, C14∶1, C16∶1, C18∶2n6c, C18∶3n3 and n-3PUFA in the longissimus dorsi muscle were correlated with the relative abundance of Megasphaera, Erysipelotrichaceae_UCG-002, Succiniclasticum and Ruminococcus (P<0.05). In conclusion, CPN can regulate the rumen microbiota structure and reduce the rumen NH3-N concentration of fattening small-tailed Han sheep. In production practice, CPN can be used as a rumen ecological regulator.

Cite this article

WANG Yuan , WANG Wenwen , YANG Yi , GAO Chang , GUO Tao , DUAN Ting , LIU Na , AN Xiaoping , QI Jingwei . Effects of Compound Plant Nutrients on Rumen Fermentation Parameters, Rumen Microbiota and Fatty Acid Composition of Longissimus dorsi Muscle in Finishing Small Tail Han Sheep[J]. Chinese Journal of Animal Nutrition, 2023 , 35(1) : 380 -390 . DOI: 10.3969/j.issn.1006-267x.2023.01.038

近些年,为了保护生态环境以及发展的需要,肉羊育肥方式已从放牧向集约化舍饲转变。在集约化快速育肥条件下,肉羊长期采食高精料饲粮,瘤胃微生物区系改变,瘤胃发酵异常,导致机体患病和肉品质下降[1]。大量科学研究已经证实,在育肥饲粮中加入植物提取物可以调控瘤胃菌群的结构,影响瘤胃发酵,促进机体健康[2]。作为在畜禽生产中广泛应用的植物提取物,丁香酚、肉桂醛以及辣椒油树脂均可调控动物肠道菌群结构,进而改善机体健康状况[3-5]。本课题组在先前的研究中已表明,发酵麸皮多糖可调控杜寒杂交肉羊瘤胃菌群结构,提高瘤胃组织中紧密连接蛋白的mRNA表达,有利于维持瘤胃健康[6]。目前关于单一营养素对肉羊瘤胃菌群结构的影响研究很多,但关于复合添加各种营养素对肉羊瘤胃菌群结构的影响研究很少。因此,本试验将发酵麸皮多糖与肉桂醛、丁香酚、辣椒油树脂等添加剂做成复合植物营养素(compound plant nutrients,CPN),添加到育肥小尾寒羊的饲粮中,旨在探究CPN对其瘤胃菌群结构、瘤胃发酵参数及背最长肌脂肪酸组成的影响,以期为CPN应用于反刍动物生产中提供理论依据。

1 材料与方法

1.1 CPN

CPN由内蒙古自治区草食家畜饲料工程技术研究中心研制,主要成分为发酵麸皮多糖(≥50%)、丁香酚(≥1.5‰)、肉桂醛(≥0.9‰)和辣椒油树脂(≥0.6‰),辅料为沸石粉等。

1.2 试验设计与饲养管理

试验选取健康且体重[(24.18±0.31) kg]相近的4月龄小尾寒羊母羊16只,并随机分为2组,每组8个重复,每个重复1只羊。对照组饲喂基础饲粮,而试验组饲喂在基础饲粮中加入了3‰ CPN的试验饲粮。基础饲粮根据《肉羊饲养标准》(NY/T 816—2004)配制,其组成及营养水平见表1。基础饲粮为全混合颗粒饲料,直径为6 mm,长度为10 mm,由内蒙古某有限公司提供。试验期为97 d,预试期7 d,正试期90 d。本试验在内蒙古巴彦淖尔市临河区肉羊试验基地进行,常规饲养管理,每日定时饲喂(08:00和17:00),每天根据前1 d的剩料量重新调整饲喂量,保证料槽中每天有10%左右的剩料。自由饮水。单栏饲养。
表1 基础饲粮组成及营养水平(风干基础)

Table 1 Composition and nutrient levels of the basal diet (air-dry basis)%

项目Items 含量Content
原料Ingredients
葵花籽壳Sunflower shell 14.00
喷浆玉米皮Shotcrete corn husk 5.00
玉米白皮Corn husk 6.00
玉米胚芽粕Corn germ meal 20.00
玉米Corn 29.20
干酒糟及其可溶物DDGS 5.00
豆粕Soybean meal 3.50
膨润土Bentonite 3.50
稻壳Rice hull 3.50
菜籽粕Rapeseed meal 2.20
糖蜜Molasses 2.00
棉籽粕Cottonseed meal 1.50
项目Items 含量Content
石粉Limestone 1.50
豆油Soybean oil 1.00
预混料Premix1) 2.10
合计Total 100.00
营养水平Nutrient levels2)
代谢能ME/(MJ/kg) 9.62
干物质DM 91.56
粗蛋白质CP 14.56
粗脂肪EE 3.95
粗灰分Ash 7.67
中性洗涤纤维NDF 38.44
酸性洗涤纤维ADF 14.92
钙Ca 0.76
磷P 0.48

1)每千克预混料含有 One kg of premix contained as follows:VA 350 000 IU,VB1 62 mg,VB2 188 mg,VB3 750 mg,VB5 500 mg,VB6 62 mg,VB7 3.7 mg,VB9 38 mg,VD3 93 750 IU,VE 938 mg,VK3 63 mg,Se 18 mg,Zn 3 000 mg,I 23 mg,Co 30 mg,Mn 2 500 mg,Fe 3 240 mg,Cu 500 mg。

2)代谢能为计算值,其他为实测值。ME was a calculated value, while the others were measured values.

1.3 样品采集

试验结束后,采用清真屠宰法屠宰所有羊只,立即收集新鲜瘤胃液,经4层纱布过滤后采集瘤胃液样本50 mL,部分用于现场测定瘤胃pH,另一部分加入4 mL 0.2 mol/L盐酸溶液混匀,用于测定瘤胃氨态氮(ammonia nitrogen, NH3-N)浓度,剩余瘤胃液用于挥发性脂肪酸(volatile fatty acid, VFA)浓度测定,-20 ℃冷冻保存。同时采集未过滤瘤胃食糜2 mL,液氮速冻,-80 ℃保存,用于瘤胃细菌Illumina-Nova测序分析。此外,取羊右侧倒数第1、2根肋骨处背最长肌样品200 g,-20 ℃冷冻保存,用于肌肉脂肪酸组成的测定。

1.4 瘤胃发酵参数的测定

瘤胃pH采用便携式酸度计(Starter 2100型,OHAUS公司,美国)测定。NH3-N浓度参照冯宗慈等[7]比色法测定。瘤胃VFA(乙酸、丙酸、异丁酸、丁酸、异戊酸和戊酸)含量采用气相色谱仪(Clarus680型,Perkin Elmer公司,美国)测定。瘤胃液样本前处理:样本解冻后,取50 μL样本,用50%甲醇稀释40倍后,再取50 μL,加入50 μL内标和50 μL衍生试剂,常温衍生30 min,加入50 μL保护剂,再加入250 μL水,涡漩振荡10 s,13 200 r/min离心10 min,取上清检测。气相色谱条件为:Elite-FFA型毛细管柱(30 m×0.25 mm);柱温120 ℃;FID检测器温度25 ℃;氮气流速30 mL/min。

1.5 Illumina-Nova测序分析

1.5.1 瘤胃食糜总DNA的提取、扩增及测序

利用Power Fecal®DNA提取试剂盒(MoBio Carlsbad,美国)提取小尾寒羊瘤胃食糜样品中微生物的总DNA,针对16S rDNA的V4区(515f:5’-GTGCCAGCMGCCGCGGTAA-3’和806r:5’-GGACTACHVGGGTWTCTAAT-3’),设计合成特异引物,进行扩增。扩增片段的测序工作由北京诺禾致源科技股份有限公司按照标准流程运用Illumina NovaSeq平台完成。

1.5.2 生物信息学分析

测序所得的原始序列,首先使用FLASH(V1.2.7)进行拼接,参照Qiime(V1.7.0)进行质量控制,得到有效序列。利用Uparse软件(v7.0.1001)对所有样品的有效序列以97%的一致性进行操作分类单元(OTU)聚类,用Mothur软件与SILVA的SSUrRNA数据库进行物种注释分析(设定阈值为0.8~1.0),在门、属水平下统计每个样品的菌群组成。各样品的数据经过均一化处理后,采用Qiime软件进行Alpha多样性和Beta多样性分析。

1.6 背最长肌脂肪酸组成的测定

小尾寒羊背最长肌脂肪酸含量采用气质联用(7890B-5977A,安捷伦公司,美国)外标法测定。气相色谱条件为:DB-23毛细管色谱柱(30 m×320 μm×0.25 μm),进样体积1 μL,进样口温度250 ℃,分流比1/5;检测器温度230 ℃,载气:氦气;柱箱温度50 ℃,1 min,25 ℃/min 到175 ℃,4 ℃/min到230 ℃,24.75 min。

1.7 统计分析

瘤胃发酵参数和背最长肌脂肪酸组成数据使用SAS 9.2软件进行t检验分析,试验结果以平均值和均值标准误(SEM)表示,而菌群数据进行非参数t检验分析。育肥小尾寒羊瘤胃菌群(属水平)与背最长肌脂肪酸含量进行Spearman相关性分析。P<0.05表示差异显著。

2 结果与分析

2.1 CPN对育肥小尾寒羊瘤胃发酵参数的影响

表2可知,与对照组相比,饲粮中添加CPN对瘤胃pH、总挥发性脂肪酸浓度、乙酸、丙酸、丁酸、异丁酸、戊酸及异戊酸的含量和乙丙比无显著影响(P>0.05),但能显著降低育肥小尾寒羊瘤胃液NH3-N浓度(P<0.05)。
表2 CPN对育肥小尾寒羊瘤胃发酵参数的影响

Table 2 Effects of CPN on rumen fermentation parameters of finishing small tail Han sheep

项目
Items
对照组
Control group
试验组
Test group
SEM P
P-value
pH 5.66 5.48 0.10 0.37
氨态氮NH3-N/(mg/dL) 11.76a 5.08b 1.80 0.04
总挥发性脂肪酸TVFA/(mmol/L) 10.58 11.97 0.57 0.24
乙酸Acetate acid/% 44.81 46.58 0.91 0.36
丙酸Propionate acid/% 35.35 37.01 1.23 0.53
异丁酸Isobutyrate acid/% 1.01 0.85 0.13 0.57
丁酸Butyrate acid/% 12.27 9.91 0.73 0.11
戊酸Valerate acid/% 3.51 3.83 0.29 0.61
异戊酸Isovalerate acid/% 0.89 0.61 0.12 0.27
乙丙比A/P 1.29 1.29 0.07 0.97

同行数据肩标不同小写字母表示差异显著(P<0.05),相同或无字母表示差异不显著(P>0.05)。下表同。

In the same row, values with different small letter superscripts mean significant difference (P<0.05), while with the same or no letter superscripts mean no significant difference (P>0.05). The same as below.

2.2 CPN对育肥小尾寒羊瘤胃菌群结构的影响

2.2.1 CPN对育肥小尾寒羊瘤胃菌群Alpha多样性指数和Beta多样性的影响
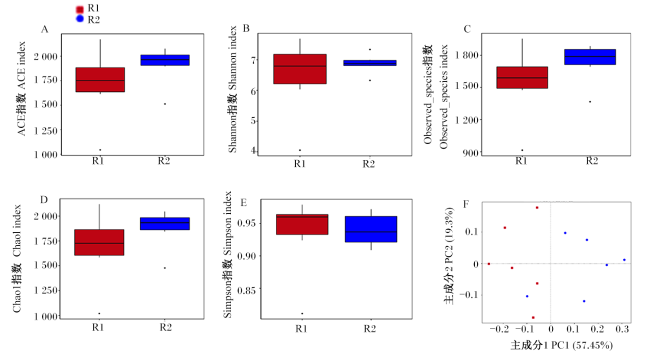
图1-A~图1-E所示,与对照组相比,添加CPN对育肥小尾寒羊瘤胃菌群Alpha多样性指数(ACE、Chao1、Observed_species、Shannon和Simpson指数)均无显著影响(P>0.05)。如图1-F显示,主成分1(PC1)的贡献率为57.45%,主成分2(PC2)的贡献率为19.30%,此结果说明对照组与试验组的瘤胃菌群结构有一定的差异。
图1 Alpha多样性和Beta多样性分析

R1:对照组;R2:试验组。下图同。

Fig.1 Analysis of Alpha and Beta diversity

R1:control group; R2: test group. The same as below.

2.2.2 CPN对育肥小尾寒羊瘤胃菌群丰度的影响

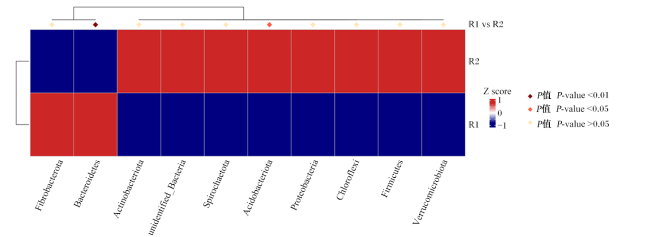
图2所示,与对照组相比,试验组瘤胃食糜中拟杆菌门(Bacteroidetes)的相对丰度显著降低(P<0.05)[44.48% vs 29.05%],酸杆菌门(Acidobacteriota)的相对丰度显著增加(P<0.05)[1.92% vs 3.10%]。
图2 MetaStat分析(门水平)

Fibrobacterota:纤维杆菌门;Bacteroidetes:拟杆菌门;Actinobacteriota:放线菌门;unidentified_Bacteria:未分类菌门;Spirochaetota:螺旋菌门;Acidobacteriota:酸杆菌门;Proteobacteria:变形菌门;Chloroflexi:绿弯菌门;Firmicutes:厚壁菌门;Verrucomicrobiota:疣微菌门。

Fig.2 MetaStat analysis (phylum level)

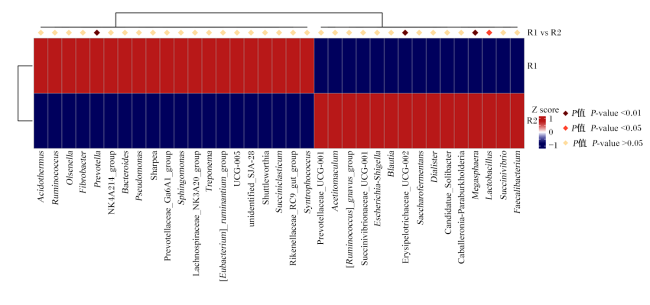
图3所示,与对照组相比,试验组瘤胃食糜中普雷沃氏菌属(Prevotella)的相对丰度显著降低(P<0.05)[33.64% vs 18.99%],而柔膜菌科UCG-002(Erysipelotrichaceae_UCG-002)[0.55% vs 1.19%]、乳杆菌属(Lactobacillus)[0.34% vs 0.87%]及巨型球菌属(Megasphaera)[0.19% vs 0.43%]的相对丰度显著增加(P<0.05)。
图3 MetaStat分析(属水平)

Acidothermus:热酸菌属;Ruminococcus:瘤胃球菌属;Olsenella:奥尔森菌属;Fibrobacter:纤维杆菌属;Prevotella:普雷沃氏菌属;Bacteroides:拟杆菌属;Pseudomonas:绿脓杆菌属;Prevotellaceae_Ga6A1_group:普雷沃氏菌科Ga6A1群;Sphingomonas:鞘氨醇单胞菌属;Lachnospiraceae_NK3A20_group:毛螺菌科NK3A20群;Treponema:密螺旋体菌属;[Eubacterium]_ruminantium_group:啮齿真杆菌属群;Succiniclasticum:解琥珀酸菌属;Rikenellaceae_RC9_gut_group:理研菌科RC9肠道群;Syntrophococcus:互营球菌属;Prevotellaceae_UCG-001:普雷沃氏菌科UCG-001;Acetitomaculum:醋酸杆菌属;[Ruminococcus]_gnavus_group:发光球菌属群;Succinivibrionaceae_UCG-001:琥珀酸弧菌科UCG-001;Escherichia-Shigella:埃希氏-志贺菌属;Blautia:布劳特氏菌属;Erysipelotrichaceae_UCG-002:柔膜菌科UCG-002;Saccharofermentans:产酸糖酵菌属;Dialister:小杆菌属;Megasphaera:巨型球菌属;Lactobacillus:乳杆菌属;Succinivibrio:琥珀酸弧菌属;Faecalibacterium:栖粪杆菌属。

Fig.3 MetaStat analysis (genus level)

2.3 CPN对育肥小尾寒羊背最长肌脂肪酸组成的影响

表3可知,试验组中育肥小尾寒羊背最长肌肉中单不饱和脂肪酸(MUFA)总量、C14∶1、C16∶1及C18∶1n9含量与对照组相比总体呈现下降趋势,分别降低了8.14%、33.33%、21.28%、7.55%,但无显著差异(P>0.05);但试验组中育肥小尾寒羊背最长肌肉中多不饱和脂肪酸 (PUFA) 总量、C18∶2n6c、C18∶3n6、C18∶3n3、C20∶2、C20∶3n6、C20∶4n6及C20∶5n3的含量与对照组相比总体呈现增加趋势,分别提高了30.77%、26.82%、27.27%、9.52%、19.05%、35.48%、51.39%,但无显著差异(P>0.05)。此外,试验组中育肥小尾寒羊背最长肌肉中n-3高度不饱和脂肪酸总量和n-6高度不饱和脂肪酸总量与对照组相比总体呈现增加趋势,分别提高了13.64%和31.53%,但无显著差异(P>0.05)。
表3 CPN对育肥小尾寒羊背最长肌脂肪酸组成的影响

Table 3 Effects of CPN on fatty acid composition of longissimus dorsi muscle of finishing small tail Han sheep%

项目
Items
对照组
Control group
试验组
Test group
SEM P
P-value
饱和脂肪酸总量Total SFA 46.08 47.13 0.926 0.594
C12∶0 0.05 0.06 0.004 0.181
C14∶0 1.97 2.13 0.128 0.554
C16∶0 26.73 26.68 0.381 0.949
C18∶0 16.48 17.17 0.741 0.665
C20∶0 0.19 0.24 0.020 0.334
C22∶0 0.41 0.55 0.075 0.395
C24∶0 0.23 0.31 0.042 0.394
单不饱和脂肪酸总量Total MUFA 45.34 41.65 1.052 0.077
C14∶1 0.06 0.04 0.008 0.488
C16∶1 1.88 1.48 0.138 0.153
C18∶1n9c 43.29 40.02 0.943 0.451
C20∶1 0.12 0.11 0.004 0.164
多不饱和脂肪酸总量Total PUFA 8.58 11.22 1.192 0.290
C18∶2n6c 6.19 7.85 0.781 0.310
C18∶3n6 0.22 0.28 0.033 0.388
C18∶3n3 0.21 0.23 0.013 0.451
C20∶2 0.21 0.25 0.027 0.475
C20∶3n6 0.31 0.42 0.057 0.364
C20∶4n6 1.44 2.18 0.293 0.222
C20∶5n3 0.02 0.02 0.003 0.400
总n-3高度不饱和脂肪酸∑n-3 PUFA 0.22 0.25 0.015 0.412
总n-6高度不饱和脂肪酸∑n-6 PUFA 8.15 10.72 1.152 0.286

2.4 育肥小尾寒羊瘤胃菌群与背最长肌脂肪酸指标之间的相关性

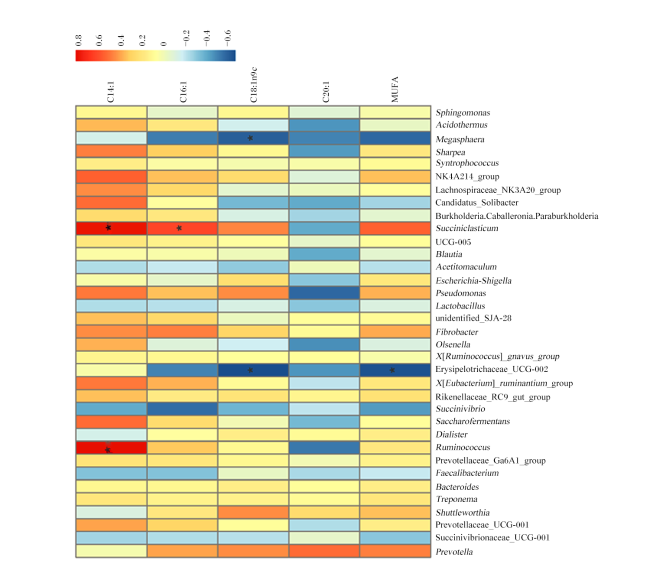
图4可知,背最长肌中C18∶1n9c含量与Megasphaera和Erysipelotrichaceae_UCG-002相对丰度呈显著负相关(P<0.05);MUFA总量与Erysipelotrichaceae_UCG-002相对丰度呈显著负相关(P<0.05);C14∶1含量与解琥珀酸菌属(Succiniclasticum)和瘤胃球菌属(Ruminococcus)相对丰度呈显著正相关(P<0.05);C16∶1含量与Succiniclasticum相对丰度呈显著正相关(P<0.05)。
图4 瘤胃菌群(属水平)与背最长肌单不饱和脂肪酸指标的相关性

MUFA:单不饱和脂肪 monounsaturated fatty acid;Sphingomonas:鞘氨醇单胞菌属;Acidothermus:热酸菌属;Megasphaera:巨型球菌属;Sharpea:夏普氏菌属;Syntrophococcus:互营球菌属;Lachnospiraceae_NK3A20_group:毛螺菌科NK4A136群;Succiniclasticum:解琥珀酸菌属;Blautia:布劳特氏菌属;Acetitomaculum:醋酸杆菌属;Escherichia-Shigella:埃希氏-志贺菌属;Pseudomonas:绿脓杆菌属;Lactobacillus:乳杆菌属;Fibrobacter:纤维杆菌属;Olsenella:奥尔森菌属;[Ruminococcus]_gnavus_group:发光球菌属群;Erysipelotrichaceae_UCG-002:柔膜菌科UCG-002;X[Eubacterium]_ruminantium_group:啮齿真杆菌属群;Rikenellaceae_RC9_gut_group:理研菌科RC9肠道群;Succinivibrio:琥珀酸弧菌属;Saccharofermentans:产酸糖酵菌属;Dialister:小杆菌属;Ruminococcus:瘤胃球菌属;Prevotellaceae_Ga6A1_group:普雷沃氏菌科Ga6A1群;Faecalibacterium:栖粪杆菌属;Bacteroides:拟杆菌属;Treponema:密螺旋体菌属;Prevotellaceae_UCG-001:普雷沃氏菌科UCG-001;Succinivibrionaceae_UCG-001:琥珀酸弧菌科UCG-001;Prevotella:普雷沃氏菌属。*表示显著相关 * mean significant correlation。下图同 the same as below。

Fig.4 Correlation between rumen bacteria (genus level) and MUFA indices in longissimus dorsi muscle

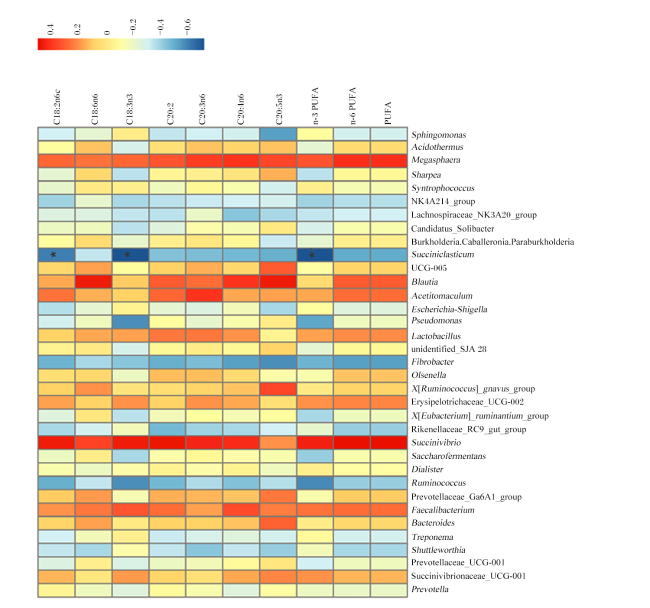
图5所知,背最长肌中C18∶2n6c、C18∶3n3及n-3PUFA含量与Succiniclasticum相对丰度呈显著负相关(P<0.05)。
图5 瘤胃菌群(属水平)与背最长肌多不饱和脂肪酸指标的相关性

PUFA:多不饱和脂肪酸polyunsaturated fatty acid。

Fig.5 Correlation between rumen bacteria (genus level) and PUFA indices in longissimus dorsi muscle

3 讨论

3.1 CPN对育肥小尾寒羊瘤胃发酵参数的影响

瘤胃pH和VFA含量是衡量瘤胃发酵状况及健康程度的重要指标[8]。本试验结果显示,饲粮中添加3‰ CPN对育肥小尾寒羊瘤胃pH、TVFA浓度、乙酸、丙酸、丁酸、异丁酸、戊酸及异戊酸含量和乙丙比均无显著影响。王金光[9]研究结果发现,添加2.5和5 g/kg的CPN均可降低杜寒杂交肉羊瘤胃中TVFA的含量,但对pH、各种VFA占比和乙丙比无显著影响。这表明CPN对小尾寒羊瘤胃pH和VFA含量无显著影响,这可能与本试验中CPN的添加剂量和肉羊品种有关,需要进一步研究。反刍动物瘤胃内的NH3-N主要是由于饲粮中的含氮化合物的脱氨基作用所形成,是反映瘤胃内氮代谢水平的主要指标之一。瘤胃内NH3-N浓度和微生物对饲粮中蛋白质的降解和利用机制相关[10]。本试验中,试验组NH3-N浓度为5.08 mg/dL,对照组为11.76 mg/dL,均在适宜范围内,且试验组NH3-N浓度低于对照组,表明饲粮中添加CPN能够提高瘤胃微生物对氮的利用速率。与本试验结果一致,Wang等[11]研究发现,作为CPN的主要成分,发酵麸皮多糖也可降低早期断奶羔羊瘤胃中NH3-N的浓度。

3.2 CPN对育肥小尾寒羊瘤胃菌群结构的影响

瘤胃菌群可以直接影响营养物质的消化利用,而饲粮是影响瘤胃菌群结构和组成的关键因素[12]。研究表明,植物提取物具有调控瘤胃菌群结构的作用[2]。本试验发现,添加CPN对育肥小尾寒羊瘤胃菌群Alpha多样性指数均无显著影响,但可影响Beta多样性,此结果说明CPN可以在一定程度上改变育肥小尾寒羊瘤胃菌群结构。在门和属水平上,添加CPN可增加Acidobacteriota、Erysipelotrichaceae_UCG-002、LactobacillusMegasphaera的相对丰度,并降低Bacteroidetes和Prevotella的相对丰度。Lactobacillus作为一种常见的益生菌,其可通过产生VFA来降低肠道pH,改善肠道菌群结构[13]Megasphaera是瘤胃中最主要的乳酸分解菌,瘤胃中超过70%以上的乳酸可被其利用,其酵解乳酸产物主要为丙酸、丁酸以及少量的乙酸和戊酸[14-15]。关于本试验发现的Acidobacteriota和Erysipelotrichaceae_UCG-002,前人研究中对其功能的描述较少,未来需要进一步探究。Erysipelotrichaceae_UCG_002属于厚壁菌门(Firmicutes)中的柔膜菌科(Erysipelotrichaceae)类,其与VFA合成密切相关[16]。基于上述研究推测,CPN组育肥小尾寒羊瘤胃中LactobacillusMegasphaera相对丰度的增加,有利于为机体提供更多的VFA,且可预防瘤胃酸中毒。研究发现,Prevotella可以产生大量的复合酶,进而可加速降解淀粉,且高淀粉饲粮会使其相对丰度增加[17-18]。本研究中,Prevotella相对丰度的减少可能是因为CPN(发酵麸皮多糖、丁香酚、肉桂醛和辣椒油树脂)的成分为非淀粉类物质,无法为Prevotella的增殖提供底物。Prevotella属于Bacteroidetes,本试验中Bacteroidetes相对丰度的降低可能主要是Prevotella的相对丰度的降低导致的。

3.3 CPN对育肥小尾寒羊背最长肌脂肪酸组成的影响

羊肉风味、嫩度和多汁性等特性主要受肌肉脂肪酸的组成和含量的影响[19]。研究表明,栗木单宁可以增加滩羊肌肉中MUFA和PUFA的含量,提高肌肉的营养价值[20]。本试验发现,CPN处理对育肥小尾寒羊背最长肌的脂肪酸组成无显著影响。郭焘等[21]试验研究表明,饲粮中添加2.5 g/kg CPN可增加杜×寒杂交母羔背最长肌中C16∶1、C17∶1、C18∶1n9c及MUFA含量,但可降低C18∶2n6c、C18∶3n6及C20∶3n6含量。试验结果不一致可能与CPN的添加剂量和肉羊品种有关,需要进一步研究。研究表明,摄食富含PUFA的肉类可通过降低胆固醇和低密度脂蛋白含量来降低心脏疾病风险[22]。本试验中,CPN添加组中背最长肌PUFA、C18∶2n6c、C18∶3n6、C18∶3n3、C20∶2、C20∶3n6、C20∶4n6及C20∶5n3的含量与对照组相比总体呈现增加趋势,这在一定程度上有利于消费者健康。Liotta等[23]研究发现,迷迭香提取物中含有的酚类物质可以终止氧化链反应并提高PUFA合成过程中Δ-5去饱和酶及Δ-6去饱和酶的活性,这可提高猪肉中PUFA的含量。因此,本试验中PUFA含量的变化可能是CPN中的丁香酚在发挥作用。

3.4 育肥小尾寒羊瘤胃菌群与背最长肌脂肪酸指标之间的相关性

羊肉中PUFA的含量与其在瘤胃内的氢化程度有关,而瘤胃菌群主要参与PUFA在瘤胃中的氢化过程[24]。本试验发现,背最长肌中C18∶1n9c含量与Megasphaera和Erysipelotrichaceae_UCG-002相对丰度呈显著负相关;MUFA总量与Erysipelotrichaceae_UCG-002相对丰度呈显著负相关;C14∶1含量与SucciniclasticumRuminococcus相对丰度呈显著正相关;C16∶1含量与Succiniclasticum相对丰度呈显著正相关;背最长肌中C18∶2n6c、C18∶3n3含量及n-3PUFA总量与Succiniclasticum相对丰度呈显著负相关。同时添加CPN可增加Erysipelotrichaceae_UCG-002和Megasphaera的相对丰度。由此推测,CPN可能通过调控育肥小尾寒羊瘤胃菌群结构,增加了Erysipelotrichaceae_UCG-002和Megasphaera的相对丰度,减少了瘤胃氢化,增加了PUFA在羊肉中的沉积。然而,关于这些变化菌种在脂肪酸代谢过程中的具体作用都还需进行深入细致的研究。

4 结论

饲粮中添加CPN可降低育肥小尾寒羊瘤胃NH3-N浓度,增加Acidobacteriota、Erysipelotrichaceae_UCG-002、LactobacillusMegasphaera的相对丰度,并降低Bacteroidetes和Prevotella的相对丰度。
[1]
ELMHADI M E, ALI D K, KHOGALI M K, et al. Subacute ruminal acidosis in dairy herds:microbiological and nutritional causes,consequences,and prevention strategies[J]. Animal Nutrition, 2022, 10:148-155.

DOI

[2]
张芮铭, 田可, 何天乐, 等. 植物提取物对高精料饲粮下反刍动物瘤胃功能、微生物区系和炎症反应的调控效果[J]. 动物营养学报, 2020, 32(1):36-41.

ZHANG R M, TIAN K, HE T L, et al. Regulation effects of plant extracts on rumen function,microflora and inflammatory response in ruminants under high-concentrate diet[J]. Chinese Journal of Animal Nutrition, 2020, 32(1):36-41. (in Chinese)

[3]
袁雯. 丁香酚对非酒精性脂肪肝病的防治作用及其微囊的制备[D]. 硕士学位论文. 青岛: 青岛科技大学, 2021.

YUAN W. Effect of eugenol on prevention and treatment of nonalcoholic fatty liver disease and preparation of its microcapsules[D]. Master’s Thesis. Qingdao: Qingdao University of Science and Technology, 2021 (in Chinese)

[4]
肖瀛, 许豪杰, 杨昌铭, 等. 肉桂精油对小鼠肝肠组织抗氧化能力以及肠道菌群结构的调节作用[J]. 食品科学, 2021, 42(7):198-206.

XIAO Y, XU H J, YANG C M, et al. Regulatory effect of cinnamon essential oil on antioxidant capacity of liver and intestine tissues and gut microbiota in mice[J]. Food Science, 2021, 42(7):198-206. (in Chinese)

[5]
LEE S, GUEVARRA R, LEE J, et al. PSX-35 effects of dietary plant extracts on growth performance and intestinal microbiota composition in weaned piglets[J]. Journal of Animal Science, 2018,96 (Suppl.3):489.

[6]
王文文, 王园, 孟子琪, 等. 发酵麸皮多糖对杜寒杂交肉羊瘤胃菌群及其屏障功能相关指标的影响[J]. 动物营养学报, 2022, 34(1):640-650.

WANG W W, WANG Y, MENG Z Q, et al. Effects of fermented wheat bran polysaccharides on microbiota and rumen barrier junction related indices of Dorper×Thin-Tailed Han crossbred meat lambs[J]. Chinese Journal of Animal Nutrition, 2022, 34(1):640-650. (in Chinese)

[7]
冯宗慈, 高民. 通过比色测定瘤胃液氨氮含量方法的改进[J]. 畜牧与饲料科学, 2010, 31(Z1):37.

FENG Z C, GAO M. Improvement on the colorimetric method of ammonia nitrogen in rumen fluid[J]. Animal Husbandry and Feed Science, 2010, 31(Z1):37. (in Chinese)

[8]
DIJKSTRA J, VAN GASTELEN S, DIEHO K, et al. Review:rumen sensors:data and interpretation for key rumen metabolic processes[J]. Animal, 2020,14 (Suppl.1):s176-s186.

[9]
王金光. 日粮添加复合营养素对肉羊生产性能、瘤胃发酵和血液指标的影响[D]. 硕士学位论文. 呼和浩特: 内蒙古农业大学, 2021.

WANG J G. Effects of compound nutrients on production performance,rumen fermentation and blood indexes of mutton sheep[D]. Master’s Thesis. Hohhot: Inner Mongolia Agricultural University, 2021 (in Chinese)

[10]
林波, 王迪铭. 反刍动物瘤胃内氨氮产生的微生物机制与调控手段[J]. 中国饲料, 2010(19):9-13.

LIN B, WANG D M. Mechanism of rumen ammonia nitrogen production and its manipulated measures[J]. China Feed, 2010(19):9-13. (in Chinese)

[11]
WANG W W, WANG Y, CUI Z W, et al. Fermented wheat bran polysaccharides intervention alters rumen bacterial community and promotes rumen development and growth performance in lambs[J]. Frontiers in Veterinary Science, 2022, 9:841406.

DOI

[12]
BELANCHE A, DOREAU M, EDWARDS J E, et al. Shifts in the rumen microbiota due to the type of carbohydrate and level of protein ingested by dairy cattle are associated with changes in rumen fermentation[J]. The Journal of Nutrition, 2012, 142(9):1684-1692.

DOI

[13]
SLOVER C M, DANZIGER L. Lactobacillus:a review[J]. Clinical Microbiology Newsletter, 2008, 30(4):23-27.

DOI

[14]
MAROUNEK M, FLIEGROVA K, BARTOS S. Metabolism and some characteristics of ruminal strains of Megasphaera elsdenii[J]. Applied and Environmental Microbiology, 1989, 55(6):1570-1573.

DOI

[15]
HENNING P H, HORN C H, STEYN D G, et al. The potential of Megasphaera elsdenii isolates to control ruminal acidosis[J]. Animal Feed Science and Technology, 2010, 157(1/2):13-19.

DOI

[16]
AHMAD A A, YANG C, ZHANG J B, et al. Effects of dietary energy levels on rumen fermentation,microbial diversity,and feed efficiency of yaks (Bos grunniens)[J]. Frontiers in Microbiology, 2020, 11:625.

DOI

[17]
ZENED A, COMBES S, CAUQUIL L, et al. Microbial ecology of the rumen evaluated by 454 GS FLX pyrosequencing is affected by starch and oil supplementation of diets[J]. FEMS Microbiology Ecology, 2013, 83(2):504-514.

DOI PMID

[18]
GARDNER R G, WELLS J E, RUSSELL J B, et al. The cellular location of Prevotella ruminicola beta-1,4-D-endoglucanase and its occurrence in other strains of ruminal bacteria[J]. Applied and Environmental Microbiology, 1995, 61(9):3288-3292.

DOI

[19]
JAVIERÁLVAREZ-RODRÍGUEZ, OLAIA U, SANDRA L, et al. Insights into the role of major bioactive dietary nutrients in lamb meat quality:a review[J]. Journal of Animal Science and Biotechnology, 2022, 13(4):951-966.

[20]
齐明江, 温红瑞, 周玉香, 等. 栗木单宁对滩羊生长性能,肉品质和肌肉脂肪酸组成的影响[J]. 动物营养学报, 2022, 34(6):3857-3866.

DOI

QI M J, WEN H R, ZHOU Y X, et al. Effects of chestnut Tannin on growth performance,meat quality and muscle fatty acid composition of Tan sheep[J]. Chinese Journal of Animal Nutrition, 2022, 34(6):3857-3866. (in Chinese)

[21]
郭焘, 胡宇超, 杨毅, 等. 复合营养素对羔羊生长性能、屠宰性能、肉品质及肌肉抗氧化能力的影响[J/OL]. 中国畜牧杂志, 2022:1-16.(2022-02-03)[2022-05-22].https://kns.cnki.net/kcms/detail/11.2083.S.20220222.1338.005.html.DOI:10.19556/j.0258-7033.20210926-03.

DOI

GUO D, HU Y C, YANG Y, et al. Effects of compound nutrients on growth performance,slaughter performance,meat quality and antioxidant index in muscle of lambs[J/OL]. Chinese Journal of Animal Science, 2022,1-16.(2022-02-03)[2022-05-22]. https://kns.cnki.net/kcms/detail/11.2083.S.20220222.1338.005.html. DOI:10.19556/j.0258-7033.20210926-03. (in Chinese)

DOI

[22]
CAO F L, ZHANG X H, YU W W, et al. Effect of feeding fermented Ginkgo biloba leaves on growth performance,meat quality,and lipid metabolism in broilers[J]. Poultry Science, 2012, 91(5):1210-1221.

DOI

[23]
LIOTTA L, CHIOFALO V, D’ALESSANDRO E, et al. Supplementation of rosemary extract in the diet of Nero siciliano pigs:evaluation of the antioxidant properties on meat quality[J]. Animal, 2015, 9(6):1065-1072.

DOI

[24]
姜雅慧, 卜登攀, 杨红建, 等. 不饱和脂肪酸在瘤胃氢化的微生物学机制研究进展[J]. 华北农学报, 2015, 30(S1):376-382.

DOI

JIANG Y H, BU D P, YANG H J, et al. The advance research of the microbial biohydrogenation mechanism of unsaturated fatty acid in rumen[J]. Acta Agriculturae Boreali-Sinica, 2015, 30(S1):376-382. (in Chinese)

Outlines

/