RESEARCH PAPER

Effects of Adding Probiotics in High Carbohydrate Diet on Growth Performance, Intestinal Digestive Enzyme and Antioxidant Enzyme Activities and Immune-Related Gene Expression of Songpu Mirror Carp (Cyprinus carpio L.)

  • LI Jinnan ,
  • FAN Ze ,
  • WU Di ,
  • WANG Liansheng , *
Expand
  • Key Open Laboratory of Cold Water Fish Germplasm Resources and Breeding of Heilongjiang Province,Heilongjiang River Fisheries Research Institute, Chinese Academy of Fishery Sciences,Harbin 150070,China
* associate professor, E-mail:

Received date: 2022-07-21

  Online published: 2023-02-13

Abstract

The purpose of this experiment was to investigate the effects of Lactobacillus acidophilusBifidobacterium animalisLactobacillus rhamnosus and Lactobacillus casei supplementation in high carbohydrate diets on growth performance and intestinal health of Songpu mirror carp (Cyprinus carpio L.). A total of 450 Songpu mirror carp with an initial body weight of (1.51±0.02) g were randomly divided into 5 groups with 3 replicates per group and 30 fish per replicate. Fish meal, casein and soybean meal were used as protein sources, and starch was used as a carbohydrate source. The carbohydrate level was 45% and the protein level was 30%. The five experimental groups were the control group (G0 group), Lactobacillus acidophilus group (G1 group), Bifidobacterium animalis group (G2 group), Lactobacillus rhamnosus group (G3 group) and Lactobacillus casein group (G4 group). The experiment lasted for 8 weeks. The results showed as follows: 1) compared with G0 group, the final weight and weight gain rate of Songpu mirror carp in G2, G3 and G4 groups were increased (P<0.05), the feed conversion ratio in G2 and G3 groups was significantly decreased (P<0.05), the viscerosomatic index, intestinal somatic index and hepatosomatic index in G2 group were the highest in all experimental groups. 2) Compared with G0 group, the whole body crude protein content in G2 group was significantly increased (P<0.05), the activities of intestinal amylase, trypsin and lipase in G2 group were significantly increased (P<0.05). 3) Compared with G0 group, all probiotics significantly decreased intestinal malondialdehyde (MDA) content (P<0.05), and increased total antioxidant capacity (T-AOC) and total superoxide dismutase (T-SOD) activity (P<0.05). Alkaline phosphatase (AKP) activity in G1, G3 and G4 groups was significantly higher than that in control group (P<0.05). Except for the G1 group, other probiotics could significantly increase nitric oxide (NO) content (P<0.05). 4) Compared with G0 group, the relative expression levels of intestinal interleukin-1β (IL-1β), interleukin-8 (IL-8) and tumor necrosis factor-α (TNF-α) genes in G1, G2 and G4 groups were significantly decreased (P<0.05). The relative expression level of interleukin-10 (IL-10) gene in G1 group was significantly increased (P<0.05). In conclusion, the supplementation of Bifidobacterium animalisLactobacillus rhamnosus and Lactobacillus casei in the high carbohydrate diet can improve the growth performance, intestinal digestive enzyme activities, antioxidant indexes and intestinal immune function of Songpu mirror carp.

Cite this article

LI Jinnan , FAN Ze , WU Di , WANG Liansheng . Effects of Adding Probiotics in High Carbohydrate Diet on Growth Performance, Intestinal Digestive Enzyme and Antioxidant Enzyme Activities and Immune-Related Gene Expression of Songpu Mirror Carp (Cyprinus carpio L.)[J]. Chinese Journal of Animal Nutrition, 2023 , 35(2) : 1123 -1133 . DOI: 10.12418/CJAN2023.106

与蛋白质和脂类相比,糖类物质是更经济、来源更广泛的能源物质,适量添加可以降低养殖成本,同时减少氮、磷排放,有利于减轻水产养殖对水环境的污染[1-2]。然而,鱼类被称为“先天性糖尿病患者”,研究表明,鱼类过多的摄入糖类物质,不仅会对其生长性能产生不利影响,也会损害肠道健康,使机体免疫功能下降,抗病力降低,严重的会导致养殖动物死亡[3-4]。在水产养殖领域,益生菌作为活体微生态制剂,因其天然、无污染等优点受到了越来越多研究者的关注[5-7]。当饲料中添加足够量的益生菌时,可以对宿主健康产生有益影响,其具有提高生长性能[8]、消化酶活性[9]、非特异性免疫功能[10]、肠道抗氧化能力[11]等功能。此外,在哺乳动物上的研究表明,摄入益生菌可以降低餐后血糖值,改善糖代谢异常[12]。但目前关于益生菌改善鱼类对饲料糖利用的研究还鲜有报道。
近年来,松浦镜鲤(Cyprinus carpio)作为培育出的优良鲤鱼品种,因其具有体表无磷、含肉率高、生长速度快等优良的经济价值,已得到了广泛的推广。Wilson[13]对鲤鱼的研究表明,其利用淀粉的能力优于葡萄糖,饲料糖的最高耐受量为40%。因此,本研究以松浦镜鲤为研究对象,探讨在高糖饲料中添加4种不同益生菌对其生长性能和肠道健康的影响,旨在寻找安全、绿色的添加剂,促进水产养殖业的健康可持续发展,为糖类物质在饲料中的高效利用奠定理论基础。

1 材料与方法

1.1 试验动物及试验饲料

松浦镜鲤选自中国水产科学院黑龙江水产研究所呼兰实验站。以鱼粉、酪蛋白、豆粕为蛋白质源,淀粉为糖源,制成糖水平为45%、蛋白质水平为30%的基础饲料,将基础饲料作为对照组(G0组),其余4组分别在基础饲料中添加有效活菌数为1×10⁸ CFU/g的嗜酸乳杆菌(Lactobacillus acidophilus)(G1组)、动物双歧杆菌(Bifidobacterium animalis)(G2组)、鼠李糖乳杆菌(Lactobacillus rhamnosus)(G3组)和干酪乳杆菌(Lactobacillus casei)(G4组)。试验饲料组成及营养水平见表1。饲料原料经粉碎过筛后,按表1配方准确称重配比,逐级充分混匀后,用双螺杆挤条机制成2 mm的颗粒饲料,制粒温度为(23±2) ℃,风干后存放于-20 ℃冰箱中备用。
表1 试验饲料组成及营养水平(风干基础)

Table 1 Composition and nutrient levels of experimental diets (air-dry basis)%

项目
Items
组别 Groups
G0 G1 G2 G3 G4
原料 Ingredients
鱼粉 Fish meal 8.0 8.0 8.0 8.0 8.0
酪蛋白 Casein 22.0 22.0 22.0 22.0 22.0
豆粕 Soybean meal 14.2 14.2 14.2 14.2 14.2
α-淀粉 α-starch 45.0 45.0 45.0 45.0 45.0
鱼油 Fish oil 1.5 1.5 1.5 1.5 1.5
豆油 Soybean oil 3.5 3.5 3.5 3.5 3.5
磷脂 Soybean lecithin 1.0 1.0 1.0 1.0 1.0
维生素预混料 Vitamin premix1) 0.3 0.3 0.3 0.3 0.3
矿物质预混料 Mineral premix2) 0.2 0.2 0.2 0.2 0.2
胆碱 Choline 0.5 0.5 0.5 0.5 0.5
磷酸二氢钙 Ca(H2PO42 2.0 2.0 2.0 2.0 2.0
蛋氨酸 Met 0.2 0.2 0.2 0.2 0.2
苯丙氨酸 Phe 1.2 1.2 1.2 1.2 1.2
苏氨酸 Thr 0.4 0.4 0.4 0.4 0.4
合计 Total 100.0 100.0 100.0 100.0 100.0
营养水平 Nutrient levels3)
粗蛋白质 Crude protein 30.66 30.87 30.57 30.71 30.77
粗脂肪 Crude lipid 6.01 6.03 6.00 6.04 6.01
无氮浸出物 NFE 45.37 45.32 45.37 45.38 45.41
水分 Moisture 11.90 11.74 11.89 12.07 12.11
粗灰分 Ash 3.15 3.17 3.14 3.14 3.17

1)维生素预混料为每千克饲料提供 Vitamin premix provided the following per kg of diets:VA 8 000 IU,VE 70 mg,VB1 18 mg,VB2 35 mg,VB6 18 mg,泛酸 pantothenate acid 60 mg,VB12 0.6 mg,VC 500 mg,VD3 2 000 IU,VK 7 mg,烟酸 niacin 200 mg,生物素 biotin 2.5 mg,叶酸 folic acid 6 mg,肌醇 inositol 1 000 mg。

2) 矿物质预混料为每千克饲料提供 Mineral premix provided the following per kg of diets:Zn 65 mg,Fe 75 mg,Cu 3.5 mg,Mn 16 mg,I 0.65 mg,Co 0.1 mg,Se 0.1 mg。

3) 营养水平为实测值。Nutrient levels were measured values.

1.2 试验设计与饲养管理

养殖试验在室内控温循环水族箱里进行,预饲2周后,选择规格均一的健康松浦镜鲤450尾,初始体重为(1.51±0.02) g,随机分为5组,每组设3个重复(30尾/缸)。每日饱食投喂3次(08:00、13:00和17:00),24 h不间断供氧,溶氧含量大于5.0 mg/L,温度为(23±1) ℃,试验周期为8周。每日吸除残饵和粪便,换1/3已曝气的水,观察并记录试验鱼摄食和死亡情况。

1.3 指标测定

1.3.1 生长性能测定

养殖试验结束后,试验鱼停食12 h,各组分别计数、称重。计算生长性能指标。
根据试验鱼体初重、末重、体长、内脏团质量、肝脏质量和肠道质量,计算增重率(weight gain rate, WGR)、饲料系数(feed conversion rate, FCR)、肥满度(condition factor,CF)、脏体指数(viscerosomatic index,VSI)、肝体指数(hepatosomatic index,HSI)和肠体指数(intestinal somatic index,ISI),具体公式如下:
增重率(%)=100×(Wt-W0)/W0
饲料系数=F/(Wt-W0);
肥满度(g/cm3)=100×W/L3
肝体指数(%)=100×Wh/W
脏体指数(%)=100×Wv/W
肠体指数(%)=100×Wi/W
式中:W0为鱼体初重(g);Wt为鱼体末重(g);F为饲料摄入量(g);W为鱼体质量(g);L为鱼体长度(cm);Wh为鱼体肝脏重(g);Wv为鱼体内脏重(g);Wi为鱼体肠道重(g)。

1.3.2 体成分测定

每个重复随机取3尾鱼,用于检测体成分。采用烘干法(105 ℃)测定鱼体水分含量(GB/T 6435—2006);采用索氏抽提法测定粗脂肪含量(GB/T 6433—2006);采用550 ℃马弗炉灼烧法测定粗灰分含量(GB/T 6438—2007);采用凯氏定氮法测量粗蛋白质含量。

1.3.3 血清生化指标测定

每个重复缸随机取6尾鱼,用MS-222麻醉后,分别称量每尾鱼的体重和体长。尾静脉取血,置于无菌离心管中,4 ℃条件下3 000 r/min离心10 min,取血清分装后存于-80 ℃冰箱保存,用于检测血清中葡萄糖(glucose,GLU)、胆固醇(cholesterol,CHOL)和甘油三酯(triglyceride,TG)含量。血清生化指标由贝克曼ProCX4全自动生化分析仪测定。

1.3.4 肠道健康指标测定

在冰盘中迅速解剖并分离内脏团并称重,然后分离肝脏并称重。最后分离肠道,剔除肠道周围脂肪和内容物,用预冷的生理盐水洗净肠道,滤纸吸干水分,测量肠道重。将其中3尾鱼的肠道存于试管中,保存于-20 ℃冰箱中用于消化酶和抗氧化酶指标的检测。另外3尾鱼的肠道迅速置于液氮中,保存于-80 ℃冰箱中用于免疫基因相对表达量的检测。

1.3.4.1 肠道消化酶和抗氧化酶活性测定

肠道消化酶的测定:样品解冻后,加入9倍体积预冷的0.86%生理盐水进行匀浆(FJ-200CL高速组织匀浆机),4 ℃条件下3 000 r/min离心10 min,取上清液分装于1.5 mL离心管中,-20 ℃保存备用。胰蛋白酶活性采用福林-酚(Folin-phenol)法测定,淀粉酶和脂肪酶活性采用南京建成生物工程研究所试剂盒测定,具体方法参见试剂盒说明书。组织蛋白含量采用考马斯亮蓝法[14]测定。
抗氧化酶活性的测定:肠道抗氧化酶活性采用南京建成生物工程研究所试剂盒,用分光光度计或酶标仪进行测定,包括丙二醛(malondialdehyde,MDA)和一氧化氮(nitric oxide,NO)含量、总抗氧化能力(total antioxidant capacity,T-AOC)及总超氧化物歧化酶(total superoxide dismutase,T-SOD)、碱性磷酸酶(alkaline phosphatase,AKP)、总一氧化氮合成酶(total nitric oxide synthase,T-NOS)活性,具体方法参见试剂盒说明书。

1.3.4.2 肠道免疫基因表达测定

肠道样品置于液氮中研磨,利用Trizol法提取肠道总RNA,测定总RNA浓度和纯度,并进行反转录合成cDNA(PrimeScript RT Master Mix,TaKaRa)。免疫相关基因的Real-time PCR特异性引物见表2,所有引物由上海英潍捷基公司合成。根据SYBR Premix Ex Taq (TaKaRa)试剂盒说明书进行免疫相关基因相对表达量的检测,采用ABI 7500 Real-time PCR仪( Applied Biosystems,美国)进行分析。反应体系为20 μL:SYBR Premix Ex Taq(2×)为10 μL,上、下游引物各0.8 μL(0.4 μmol/L),ROX Reference Dye Ⅱ(50×)0.4 μL,cDNA模板2 μL,补ddH2O至20 μL。β-肌动蛋白(β-actin)作为内参基因,使用2-ΔΔCt方法[15]进行数据分析,数据取3次重复的平均值。
表2 免疫相关基因引物

Table 2 Primers of immune-related genes

基因名称
Gene names
引物序列
Primer sequence (5'—3')
登录号
Accession number
肿瘤坏死因子-α
TNF-α
F:AAGTCTCAGAACAATCAGGAA
R:TGCCTTGGAAGTGACATT
AJ311800
白细胞介素-1β
IL-1β
F:AACTTCACACTTGAGGAT
R:GACAGAACAATAACAACAAC
KC008576
白细胞介素-8
IL-8
F:AAACTGAGAGTCGACGCATTG
R:TTTTCAATGACCTTCTTAACCCAG
EU011243.1
白细胞介素-10
IL-10
F:GCCAGCATAAAGAACTCG
R:CCAAATACTGCTCGATGT
JX524551.1
转化生长因子-β2
TGF-β2
F:GGGACATCATCGCCATCT
R:TGACATTCTCGGCAGGGT
U66874.1
β-肌动蛋白
β-actin
F:GGCAGGTCATCACCATCGG
R:TTGGCATACAGGTCTTTACGG
JQ619774.1

1.4 统计分析

数据用平均值±标准差表示,利用SPSS 19.0统计软件进行单因素方差分析和Duncan氏法多重比较,P<0.05表示差异显著。

2 结果

2.1 高糖饲料中添加不同益生菌对松浦镜鲤生长性能和血清生化指标的影响

表3可知,与G0组相比,除G1组外,G2、G3和G4组松浦镜鲤的末重和增重率均显著提高(P<0.05),G2和G3组饲料系数显著降低(P<0.05);各组间肥满度没有显著差异(P>0.05);G2组的脏体指数、肠体指数和肝体指数为各试验组中最高,各添加组与对照组相比差异不显著(P>0.05)。
表3 高糖饲料中添加不同益生菌对松浦镜鲤生长性能的影响

Table 3 Effects of different probiotics in high carbohydrate diet on growth performance of Songpu mirror carp

项目
Items
组别 Groups
G0 G1 G2 G3 G4
初重 IBW/g 1.52±0.03 1.51±0.01 1.52±0.01 1.51±0.01 1.52±0.02
末重 FBW/g 5.83±0.14a 6.14±0.12ab 6.39±0.05b 6.32±0.05b 6.37±0.15b
增重率 WGR/% 290.76±26.13a 286.31±9.02a 323.41±5.11b 318.18±3.84b 322.11±10.45b
饲料系数 FCR 1.41±0.11b 1.47±0.08b 1.20±0.05a 1.19±0.01a 1.39±0.03ab
肥满度 CF/(g/cm3 3.09±0.41 2.96±0.19 3.11±0.44 2.95±0.31 3.25±0.56
脏体指数 VSI/% 12.92±1.85ab 11.70±2.96ab 13.64±2.18b 11.75±2.54ab 11.12±2.29a
肠体指数 ISI/% 4.21±0.87ab 3.86±1.06a 4.96±1.19b 4.51±0.80ab 4.70±0.93ab
肝体指数 HSI/% 7.90±2.02ab 5.55±1.80a 9.26±2.44b 6.51±3.00a 6.20±2.87a

同行数据肩标无字母或相同字母表示差异不显著(P>0.05),不同小写字母表示差异显著(P<0.05)。下表同。

In the same row, values with no letter or the same letter superscripts mean no significant difference (P>0.05), while with different small letter superscripts mean significant difference (P<0.05). The same as below.

表4可知,G3组的血清GLU含量显著低于G0组(P<0.05),其他各组间血清GLU含量没有显著差异(P>0.05)。血清CHOL和TG含量各组间没有显著差异(P>0.05)。
表4 高糖饲料中添加不同益生菌对松浦镜鲤血清生化指标的影响

Table 4 Effects of different probiotics in high carbohydrate diet on serum biochemical indices of Songpu mirror carpmmol/L

项目
Items
组别 Groups
G0 G1 G2 G3 G4
葡萄糖 GLU 7.95±0.75a 7.69±1.46a 7.00±0.92ab 5.41±0.83b 6.73±1.21ab
胆固醇 CHOL 4.74±0.40 4.31±0.43 5.75±1.11 4.40±0.30 4.68±1.07
甘油三酯 TG 8.01±0.84 8.62±0.20 8.46±0.57 8.14±0.63 7.52±0.51

2.2 高糖饲料中添加不同益生菌对松浦镜鲤体成分的影响

表5可知,与G0组和G2组相比,G4组全鱼的水分含量显著提高(P<0.05),粗脂肪含量显著降低(P<0.05);G2组全鱼粗蛋白质含量与G0组相比显著增加(P<0.05)。各组间粗灰分含量差异不显著(P>0.05)。
表5 高糖饲料中添加不同益生菌对松浦镜鲤体成分的影响

Table 5 Effects of different probiotics in high carbohydrate diet on composition of whole body of Songpu mirror carp%

项目
Items
组别 Groups
G0 G1 G2 G3 G4
水分 Moisture 71.06±0.79a 71.47±0.53ab 70.88±0.65a 71.54±0.62ab 72.65±0.53b
粗蛋白质 Crude protein 12.48±0.29ab 12.75±0.83b 14.10±0.13c 12.13±0.23ab 11.68±0.39a
粗脂肪 Crude lipid 12.79±0.47b 11.63±0.46ab 12.18±1.00b 11.70±0.17ab 10.54±1.06a
粗灰分 Ash 2.94±0.08 2.73±0.45 3.00±0.19 3.12±0.17 2.71±0.35

2.3 高糖饲料中添加不同益生菌对松浦镜鲤肠道消化酶活性的影响

表6可知,与G0组相比,G2组肠道淀粉酶、胰蛋白酶和脂肪酶活性显著增加(P<0.05);G1和G3组肠道淀粉酶活性显著高于G0组(P<0.05)。
表6 高糖饲料中添加益生菌对松浦镜鲤肠道消化酶活性的影响

Table 6 Effects of different probiotics in high carbohydrate diet on intestinal digestive enzyme activities of Songpu mirror carp

项目
Items
组别 Groups
G0 G1 G2 G3 G4
淀粉酶 Amylase/(U/g prot) 24.95±1.46a 40.70±3.27bc 50.28±7.14c 45.40±5.02bc 34.78±1.49ab
胰蛋白酶
Trypsin/(U/mg prot)
4 598.76±359.87a 4 695.58±145.72a 5 830.94±127.65b 4 155.91±263.35a 4 525.36±669.26a
脂肪酶 Lipase/(U/g prot) 5.52±0.43a 8.07±1.66a 12.08±1.99b 6.59±0.12a 5.68±0.54a

2.4 高糖饲料中添加不同益生菌对松浦镜鲤肠道抗氧化酶活性的影响

表7可知,与G0组相比,各添加组肠道MDA含量均显著降低(P<0.05),同时显著增加肠道T-AOC(P<0.05),提高T-SOD活性(P<0.05)。G1、G3和G4组肠道AKP活性显著高于G0组(P<0.05)。G2、G3和G4组肠道NO含量显著高于G0组(P<0.05);G3和G4组肠道T-NOS活性显著高于G0组(P<0.05)。
表7 高糖饲料中添加不同益生菌对松浦镜鲤肠道抗氧化酶活性的影响

Table 7 Effects of different probiotics in high carbohydrate diet on intestinal antioxidant enzyme activities of Songpu mirror carp

项目
Items
组别 Groups
G0 G1 G2 G3 G4
丙二醛
MDA/(nmol/mg prot)
83.78±1.08c 69.47±6.23b 57.61±7.07b 39.93±4.32a 57.86±9.27b
总抗氧化能力
T-AOC/(U/mg prot)
0.12±0.02a 0.47±0.06b 0.27±0.06b 0.67±0.06c 0.38±0.05b
总超氧化物歧化酶
T-SOD/(U/mg prot)
23.06±0.75a 25.76±0.19b 28.39±1.19c 26.61±2.43b 26.41±1.92b
碱性磷酸酶
AKP/(金氏单位/g prot)
576.41±39.20a 869.53±98.89c 664.04±27.41ab 819.26±95.02bc 910.85±48.92c
一氧化氮
NO/(μmol/g prot)
0.55±0.12a 0.68±0.29a 1.31±0.17b 1.79±0.13c 1.55±0.19bc
总一氧化氮合成酶
T-NOS/(U/mg prot)
2.64±0.03a 3.01±0.27ab 2.62±0.01a 3.37±0.24b 3.56±0.56b

2.5 高糖饲料中添加不同益生菌对松浦镜鲤肠道免疫基因相对表达量的影响

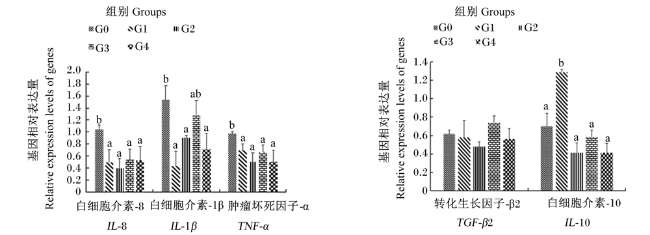
图1可知,与G0组相比,各添加益生菌的试验组促炎因子白细胞介素-8(IL-8)和肿瘤坏死因子-α (TNF-α)基因相对表达量显著降低(P<0.05);除G3组外,其余益生菌添加组促炎因子白细胞介素-1β(IL-1β)基因相对表达量显著降低(P<0.05);转化生长因子-β2(TGF-β2)基因相对表达量在各试验组间没有显著差异(P>0.05),G1组的白细胞介素-10(IL-10)基因相对表达量显著高于其他各组(P<0.05)。
图1 高糖饲料中添加不同益生菌对松浦镜鲤肠道免疫基因相对表达量的影响

数据柱形标注不同小写字母表示差异显著(P<0.05)。

Fig.1 Effects of different probiotics in high carbohydrate diet on relative expression levels of intestinal immune-related genes of Songpu mirror carp

Value columns with different small letters mean significant difference (P<0.05).

3 讨论

3.1 高糖饲料中添加益生菌对松浦镜鲤生长性能的影响

本试验结果显示,高糖饲料中添加1×10⁸ CFU/g的动物双歧杆菌、鼠李糖乳杆菌、干酪乳杆菌均可以显著提高松浦镜鲤的末重和增重率,同时,饲料中添加动物双歧杆菌和鼠李糖乳杆菌显著降低了饲料系数。饲料中添加益生菌可以提高动物的生长性能,在牙鲆(Paralichthys olivaceus[16]、大菱鲆(Scophthalmus maximus L.)[17]、锦鲤(Cyprinus carpio[18]、黑鲷(Sparus macrocephlus[19]、尼罗罗非鱼(Oreochromis niloticus[20]等水产动物上都有研究。但是,在本试验中,添加嗜酸乳杆菌对松浦镜鲤的生长性能没有显著影响,这一结果与大菱鲆[17]的研究结果类似,其研究显示添加嗜酸乳杆菌对养殖初期或中期的鱼体增重率有显著的影响,但在养殖后期增重率显著下降。吴志宏等[17]研究认为,其原因可能是过量添加嗜酸乳杆菌导致了鱼体内菌群结构失调,影响了鱼类的生长性能,或者是由于嗜酸乳杆菌在消化道内产生了过量的酶,抑制了体内内源酶的活性,降低了对营养物质的吸收作用,从而抑制了生长性能。李军亮等[21]在斜带石斑鱼(Epinephelus coioides)幼鱼的研究中也发现,过量的添加嗜酸乳杆菌会降低生长性能。本试验中,除嗜酸乳杆菌没有提高松浦镜鲤生长性能外,其余3种益生菌均显著提高了松浦镜鲤的生长性能,其可能的原因是与嗜酸乳杆菌的添加剂量或投喂方式有关,需要进一步试验的验证。
鱼体的体成分可以反映鱼体对饲料营养物质的利用情况。本试验结果显示,饲料中添加动物双歧杆菌显著增加全鱼粗蛋白质的含量,这一结果与Sahandi等[22]和Mohapatra等[23]的研究结果一致。

3.2 高糖饲料中添加益生菌对松浦镜鲤消化吸收能力的影响

鲤鱼作为无胃鱼,肠道是其营养物质的主要吸收和消化的场所,肠道中分泌的消化酶活性则是衡量其消化能力的重要指标。本试验结果显示,高糖饲料中添加嗜酸乳杆菌、动物双歧杆菌和鼠李糖乳杆菌均显著增加肠道中消化酶的活性,这一结果与Mohapatra等[23]在南亚野鲮(Labeo rohita)中的研究结果一致。动物双歧杆菌组肠道胰蛋白酶活性的增加提高了蛋白质消化能力,从而提高鱼体的生长性能和全鱼粗蛋白质的含量。李军亮等[21]对斜带石斑鱼的研究表明,其肠道消化酶活性及相关酶mRNA表达量随饲料中嗜酸乳杆菌的添加量增加呈先升高后降低的趋势。本试验高糖饲料中添加干酪乳杆菌并未改善肠道消化酶活性,其原因可能与其添加剂量有关。

3.3 高糖饲料中添加益生菌对松浦镜鲤肠道抗氧化功能的影响

抗氧化系统由1组抗氧化酶和1组低分子质量分子组成[24-26]。这种防御系统的重要组成部分是T-AOC、SOD和MDA等。MDA是脂质过氧化的产物,其含量的高低是细胞损伤程度的标志[27]。本试验中,各益生菌添加组肠道MDA含量显著降低,肠道T-AOC和T-SOD活性提高。有研究表明,过量的碳水化合物会导致鱼类持续高血糖,最终导致慢性应激[28],Zhao等[29]对大口黑鲈(Micropterus salmoides)的研究也表明,长时间的高糖摄入,会导致肠道抗氧化能力的降低。本试验结果说明,高糖饲料中添加适宜水平的益生菌可提高肠道的抗氧化能力,降低氧化损伤。赵瑞祯等[30]在刺参(Stichopus japonicus)的研究中表明,益生菌组肠道MDA含量显著降低, SOD活性提高。AKP是机体免疫抗病必不可少的免疫酶[31],研究表明,其活性高低与鱼体的抗病力呈正相关[32]。本研究中,添加嗜酸乳杆菌、鼠李糖乳杆菌和干酪乳杆菌均显著提高肠道AKP活性。李咏梅等[33]在凡纳滨对虾(Litopenaeus vannamei)的研究中也得到相似的结果。T-NOS在机体免疫物质诱导下会释放大量的NO,生成的NO在机体免疫系统中的作用十分重要[34]。本试验结果显示,高糖饲料中添加动物双歧杆菌、鼠李糖乳杆菌和干酪乳杆菌显著提高肠道NO的含量,说明益生菌可以通过提高机体的NO含量来提高机体的免疫功能。

3.4 高糖饲料中添加益生菌对松浦镜鲤免疫指标的影响

细胞因子是免疫细胞分泌的一种不可或缺的调节因子,具有调节免疫应答、修复受损组织和抵御感染等功能[35]。TNF-α、IL-1β、IL-8等促炎细胞因子在鱼类肠道免疫反应中发挥重要作用,是评估肠道炎症的重要标志物[36]。IL-10和TGF-β是多效抗炎因子,通过抑制炎症细胞因子的释放来有效缓解炎症[37]。研究表明,长时间饲喂高碳水化合物饲料会导致促炎因子TNF-αIL-1βIL-8的表达量增加,因而导致大口黑鲈[29]、团头鲂(Megalobrama amblycephala[36]、牙鲆[38]和杂交石斑鱼(Epinephelus fuscoguttatus♀×E. lanceolatus♂)[39]发生炎症反应。本试验的结果显示,高糖饲料中添加益生菌可显著降低这些促炎因子的表达量,添加嗜酸益生菌显著提高抗炎因子IL-10的相对表达量,而TGF-β2基因相对表达量并没有受到益生菌的影响。这些结果与Feng等[10]在鲤鱼上的研究结果一致,添加乳酸菌可抑制促炎因子TNF-αIL-1β基因的表达,促进抗炎因子IL-10和TGF-β基因的表达。然而,一些学者在对乌鳢(Channa argus[40]、牙鲆[41-42]、罗非鱼[43]等的研究发现,饲料中添加益生菌会同时上调抗炎因子和促炎因子的表达。这些不一致的结果可能与益生菌的种类或用量相关,其相关的机制值得进一步的研究和探讨。

4 结论

综上所述,在高糖饲料中添加动物双歧杆菌、鼠李糖乳杆菌、干酪乳杆菌可以显著提高松浦镜鲤生长性能,同时提高肠道消化酶活性及抗氧化指标,以及肠道免疫功能。
[1]
LI X Y, ZHENG S X, MA X K, et al. Effects of dietary starch and lipid levels on the protein retention and growth of largemouth bass (Micropterus salmoides)[J]. Amino Acids, 2020, 52(6/7):999-1016.

DOI

[2]
CASTRO C, PERÉZ-JIMÉNEZ A, COUTINHO F, et al. Dietary carbohydrate and lipid sources affect differently the oxidative status of European sea bass (Dicentrarchus labrax) juveniles[J]. British Journal of Nutrition, 2015, 114(10):1584-1593.

DOI

[3]
ZHOU Y L, HE G L, JIN T, et al. High dietary starch impairs intestinal health and microbiota of largemouth bass,Micropterus salmoides[J]. Aquaculture, 2021, 534:736261.

DOI

[4]
LI M, HU F C, QIAO F, et al. Sodium acetate alleviated high-carbohydrate induced intestinal inflammation by suppressing MAPK and NF-κB signaling pathways in Nile tilapia (Oreochromis niloticus)[J]. Fish & Shellfish Immunology, 2020, 98:758-765.

[5]
MAAS R M, VERDEGEM M C J, DEBNATH S, et al. Effect of enzymes (phytase and xylanase),probiotics (B. amyloliquefaciens) and their combination on growth performance and nutrient utilisation in Nile tilapia[J]. Aquaculture, 2021, 533:736226.

DOI

[6]
KHAN M I R, CHOUDHURY T G, KAMILYA D, et al. Characterization of Bacillus spp. isolated from intestine of Labeo rohita—towards identifying novel probiotics for aquaculture[J]. Aquaculture Research, 2020, 52(2):822-830.

DOI

[7]
BACK S J, PARK S J, MOON J S, et al. The effects of dietary heat-killed probiotics bacteria additives in low-fishmeal feed on growth performance,immune responses,and intestinal morphology in juvenile olive flounder Paralichthys olivaceus[J]. Aquaculture Reports, 2020, 18:100415.

DOI

[8]
ZHANG J J, YANG H L, YAN Y Y, et al. Effects of fish origin probiotics on growth performance,immune response and intestinal health of shrimp (Litopenaeus vannamei) fed diets with fish meal partially replaced by soybean meal[J]. Aquaculture Nutrition, 2020, 26(4):1255-1265.

DOI

[9]
GHANEI-MOTLAGH R, MOHAMMADIAN T, GHARIBI D, et al. Quorum quenching probiotics modulated digestive enzymes activity,growth performance,gut microflora,haemato-biochemical parameters and resistance against Vibrio harveyi in Asian seabass (Lates calcarifer)[J]. Aquaculture, 2021, 531:735874.

DOI

[10]
FENG J C, CHANG X L, ZHANG Y R, et al. Effects of lactococcus lactis from Cyprinus carpio L. as probiotics on growth performance,innate immune response and disease resistance against Aeromonas hydrophila[J]. Fish & Shellfish Immunology, 2019, 93:73-81.

[11]
YANG G, CAO H Z, JIANG W H, et al. Dietary supplementation of Bacillus cereus as probiotics in Pengze crucian carp (Carassius auratus var. Pengze):effects on growth performance,fillet quality,serum biochemical parameters and intestinal histology[J]. Aquaculture Research, 2019, 50(8):2207-2217.

DOI

[12]
郑晗盈, 兰慧, 庄滢滢, 等. 动物双歧杆菌和罗伊氏乳杆菌改善肥胖小鼠糖脂代谢异常的研究[J]. 营养学报, 2021, 43(3):283-288.

ZHENG H Y, LAN H, ZHUANG Y Y, et al. Effects of Bifidobacterium cp-9 and Lactobacillus reuteri on glucose and lipid metabolism in obese mice[J]. Acta Nutrimenta Sinica, 2021, 43(3):283-288. (in Chinese)

[13]
WILSON R P. Utilization of dietary carbohydrate by fish[J]. Aquaculture, 1994, 124(1/2/3/4):67-80.

DOI

[14]
李晋南, 王常安, 张圆圆, 等. 高淀粉水平下精氨酸对松浦镜鲤肠道形态与功能的影响[J]. 广东海洋大学学报, 2021, 41(1):39-46.

LI J N, WANG C A, ZHANG Y Y, et al. Effect of arginine supplementation in high starch diets on intestinal digestive enzyme activities and intestinal morphology of Songpu mirror carp (Cyprinus carpio L.)[J]. Journal of Guangdong Ocean University, 2021, 41(1):39-46. (in Chinese)

[15]
LI J N, ZHANG Y Y, FAN Z, et al. Effects of arginine and/or N-carbamylglutamate supplementation on growth,biochemical composition and expression of growth-regulating factors of hybrid sturgeon (Acipenser schrenckii♀×A. baerii♂) juveniles fed an arginine-deficient diet[J]. Animal Feed Science and Technology, 2022, 285:115246.

DOI

[16]
GATESOUPE F J. The effect of three strains of lactic bacteria on the production rate of rotifers,Brachionus plicatilis,and their dietary value for larval turbot,Scophthalmus maximus[J].Aquaculture, 1991, 96(3/4):335-342.

[17]
吴志宏, 王颖, 胡凡光, 等. 嗜酸乳杆菌对大菱鲆生长促进作用的研究[J]. 渔业现代化, 2013, 40(4):28-31,50.

WU Z H, WANG Y, HU F G, et al. Study on the effect of Lactobacillus acidophilus on promoting growth of turbot Scophthalmus maximus (Linnaeus)[J]. Fishery Modernization, 2013, 40(4):28-31,50. (in Chinese)

[18]
史东杰, 李文通, 姜巨峰, 等. 益生菌对锦鲤幼鱼生长性能及血液、肝脏和肠道组织中相关免疫基因表达的影响[J]. 动物医学进展, 2021, 42(5):36-41

SHI D J, LI W T, JIANG J F, et al. Effects of probiotics on growth and blood,liver and intestinal tissue immune related gene expressions of juvenile Koi carp (Cyprinus carpio)[J]. Progress in Veterinary Medicine. 2021, 42(5):36-41. (in Chinese)

[19]
SUZER C, ÇOBAN D, KAMACI H O, et al. Lactobacillus spp. bacteria as probiotics in gilthead sea bream (Sparus aurata,L.) larvae:effects on growth performance and digestive enzyme activities[J]. Aquaculture, 2008, 280(1/2/3/4):140-145.

DOI

[20]
LARA-FLORES M, OLVERA-NOVOA M A, GUZMÁN-MÉNDEZ B E, et al. Use of the bacteria Streptococcus faecium and Lactobacillus acidophilus,and the yeast Saccharomyces cerevisiae as growth promoters in Nile tilapia (Oreochromis niloticus)[J]. Aquaculture, 2003, 216(1/2/3/4):193-201.

DOI

[21]
李军亮, 杨奇慧, 谭北平, 等. 嗜酸乳杆菌对斜带石斑鱼幼鱼生长、消化性能和抗病力的影响[J]. 水生生物学报, 2019, 43(5):992-1000.

LI J L, YANG Q H, TAN B P, et al. Effects of Lactobacillus acidophilus (gim:1.730) on growth,digestive capacity,disease resistance of juvenile,Epinephelus coioides[J]. Acta Hydrobiologica Sinica, 2019, 43(5):992-1000. (in Chinese)

[22]
SAHANDI J, JAFARYAN H, SOLTANI M, et al. The use of two Bifidobacterium strains enhanced growth performance and nutrient utilization of rainbow trout (Oncorhynchus mykiss) fry[J]. Probiotics and Antimicrobial Proteins, 2019, 11(3):966-972.

DOI

[23]
MOHAPATRA S, CHAKRABORTY T, PRUSTY A K, et al. Use of different microbial probiotics in the diet of rohu,Labeo rohita fingerlings:effects on growth,nutrient digestibility and retention,digestive enzyme activities and intestinal microflora[J]. Aquaculture Nutrition, 2012, 18(1):1-11.

DOI

[24]
AHMAD I, HAMID T, FATIMA M, et al. Induction of hepatic antioxidants in freshwater catfish (Channa punctatus Bloch) is a biomarker of paper mill effluent exposure[J]. Biochimica et Biophysica Acta (BBA):General Subjects, 2000, 1523(1):37-48.

DOI

[25]
DÍAZ M E, FURNÉ M, TRENZADO C E, et al. Antioxidant defences in the first life phases of the sturgeon Acipenser naccarii[J]. Aquaculture, 2010, 307(1/2):123-129.

DOI

[26]
OU M M, WANG Y, CAI W M. Physiological and biochemical changes in Microcystis aeruginosa Qutz. in phosphorus limitation[J]. Journal of Integrative Plant Biology, 2005, 47(6):692-702.

DOI

[27]
DAWOOD M A O, KOSHIO S, EL-SABAGH M, et al. Changes in the growth,humoral and mucosal immune responses following β-glucan and vitamin C administration in red sea bream,Pagrus major[J]. Aquaculture, 2017, 470:214-222.

DOI

[28]
HEMRE G I, MOMMSEN T P, KROGDAHL Å. Carbohydrates in fish nutrition:effects on growth,glucose metabolism and hepatic enzymes[J]. Aquaculture Nutrition, 2002, 8(3):175-194.

DOI

[29]
ZHAO L L, LIANG J, CHEN F K, et al. High carbohydrate diet induced endoplasmic reticulum stress and oxidative stress,promoted inflammation and apoptosis,impaired intestinal barrier of juvenile largemouth bass (Micropterus salmoides)[J]. Fish & Shellfish Immunology, 2021, 119:308-317.

[30]
赵瑞祯, 张健. 益生菌对刺参生长性能、肠道酶活性及抗氧化性能的影响[J]. 中国饲料, 2021(20):61-64.

ZHAO R Z, ZHANG J. Effects of probiotics on growth performance,intestinal enzyme activities and anti-oxidation of Stichopus japonicus[J]. China Feed, 2021(20):61-64. (in Chinese)

[31]
高三玉. 益生菌的作用机理及在动物生产中应用[J]. 中国畜牧兽医文摘, 2014, 30(4):185-187.

GAO S Y. Mechanism of probiotics and its application in animal production[J]. Chinese Abstracts of Animal Husbandry and Veterinary Medicine, 2014, 30(4):185-187. (in Chinese)

[32]
SHIRAZI S P, BEECHEY R B, BUTTERWORTH P J. The use of potent inhibitors of alkaline phosphatase to investigate the role of the enzyme in intestinal transport of inorganic phosphate[J]. Biochemical Journal, 1981, 194(3):803-809.

PMID

[33]
李咏梅, 李腾飞, 田相利, 等. 添加益生菌和PHBV对凡纳滨对虾养殖系统水质和对虾生长、非特异免疫指标的影响[J]. 中国海洋大学学报(自然科学版), 2021, 51(11):22-31.

LI Y M, LI T F, TIAN X L, et al. Effects of probiotics and polyhydroxybutyrate on growth and non-specific immunity of Litopenaeus vannamei and its culturing water quality[J]. Periodical of Ocean University of China (Natural Science Edition), 2021, 51(11):22-31. (in Chinese)

[34]
王广军, 谢骏, 余德光, 等. 一氧化氮及一氧化氮合酶在水生动物免疫系统中的研究进展[J]. 水产科技,20093):1-6,13.

WANG G J, XIE J, YU D G, et al. The advances of the nitric oxide and nitric oxide synthase in immune system of aquatic animals[J]. Fisheries Science & Technology, 2009(3):1-6,13. (in Chinese)

[35]
CHEN S W, LIU C H, HU S Y. Dietary administration of probiotic Paenibacillus ehimensis NPUST1 with bacteriocin-like activity improves growth performance and immunity against Aeromonas hydrophila and Streptococcus iniae in Nile tilapia (Oreochromis niloticus)[J]. Fish & Shellfish Immunology, 2019, 84:695-703.

[36]
XU C, LIU W B, REMØ S C, et al. Feeding restriction alleviates high carbohydrate diet-induced oxidative stress and inflammation of Megalobrama amblycephala by activating the AMPK-SIRT1 pathway[J]. Fish & Shellfish Immunology, 2019, 92:637-648.

[37]
ALY S M, ABDEL-GALIL AHMED Y, ABDEL-AZIZ GHAREEB A, et al. Studies on Bacillus subtilis and Lactobacillus acidophilus,as potential probiotics,on the immune response and resistance of Tilapia nilotica (Oreochromis niloticus) to challenge infections[J]. Fish & Shellfish Immunology, 2008, 25(1/2):128-136.

[38]
DENG K Y, PAN M Z, LIU J H, et al. Chronic stress of high dietary carbohydrate level causes inflammation and influences glucose transport through SOCS3 in Japanese flounder Paralichthys olivaceus[J]. Scientific Reports, 2018, 8(1):7415.

DOI

[39]
LI S L, WANG A, LI Z Q, et al. Antioxidant defenses and non-specific immunity at enzymatic and transcriptional levels in response to dietary carbohydrate in a typical carnivorous fish,hybrid grouper (Epinephelus fuscoguttatus♀×E. lanceolatus♂)[J]. Fish & Shellfish Immunology, 2020, 100:109-116.

[40]
KONG Y D, GAO C S, DU X Y, et al. Effects of single or conjoint administration of lactic acid bacteria as potential probiotics on growth,immune response and disease resistance of snakehead fish (Channa argus)[J]. Fish & Shellfish Immunology, 2020, 102:412-421.

[41]
KIM D, BECK B R, HEO S B, et al. Lactococcus lactis BFE920 activates the innate immune system of olive flounder (Paralichthys olivaceus),resulting in protection against Streptococcus iniae infection and enhancing feed efficiency and weight gain in large-scale field studies[J]. Fish & Shellfish Immunology, 2013, 35(5):1585-1590.

[42]
HASAN M T, JANG W J, TAK J Y, et al. Effects of Lactococcus lactis subsp. lactis I2 with β-glucooligosaccharides on growth,innate immunity and streptococcosis resistance in olive flounder (Paralichthys olivaceus)[J]. Journal of Microbiology and Biotechnology, 2018, 28(9):1433-1442.

DOI

[43]
LIU W S, REN P F, HE S X, et al. Comparison of adhesive gut bacteria composition,immunity,and disease resistance in juvenile hybrid tilapia fed two different Lactobacillus strains[J]. Fish & Shellfish Immunology, 2013, 35(1):54-62.

Outlines

/