

1 PACs的结构与来源
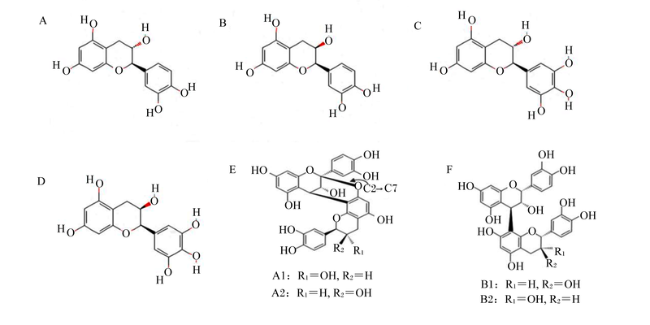
图1 PACs单体和二聚体化学结构示例A:(+)-儿茶素 (+)-catechin;B:(-)-表儿茶素 (-)-epicatechin;C:(+)-没食子儿茶素 (+)-gallocatechin;D:(-)-表没食子儿茶素 (-)-epigallocatechin;E:A型原花青素 A-type proanthocyanidins;F:B型原花青素 B-type proanthocyanidins。 A~D引自文献[5],E和F引自文献[3]。A to D were cited from literature [5], and E and F were cited from literature [3]. Fig.1 Example of chemical structures of PACs monomer and dimer[6] |
2 PACs通过对肠道菌群的重塑及其代谢产物参与调节免疫应答
2.1 PACs对肠道菌群的重塑调节免疫应答
2.2 PACs对肠道菌群代谢产物的干预影响免疫应答
2.2.1 SCFAs、胆汁酸和吲哚
2.2.2 PACs经肠道菌群生物转化的代谢物
3 PACs通过肠道菌群及其代谢产物调节免疫应答的作用机制
3.1 PACs通过肠道嗜黏蛋白阿克曼菌调节免疫应答
表1 PACs对肠道菌群及代谢产物的调节作用(以葡萄和葡萄籽来源PACs为例)Table 1 Regulatory effects of PACs on intestinal microbiota and their metabolites (a case study on grape and grape seed source PACs) |
| PACs来源 PACs sources | 动物种类 Animal species | 研究模型 Research model | 每日剂量 Daily dosage | 调节作用 Regulatory effects | 参考文献 References |
|---|---|---|---|---|---|
| 葡萄 Grape | C57BL/6J小鼠 | HFHS饲粮 | 1% DM | 粪便和盲肠菌群的丰富度降低,多样性不变,厚壁菌门 丰度降低,疣微菌门的阿克曼菌丰度提高 | [26] |
| 葡萄籽 Grape seed | C57BL/6J小鼠 | HFHS饲粮 | 300 mg/kg BW 500 mg/kg BW | 显著改变肠道菌群结构β多样性,普雷沃菌属、ⅩⅣa梭状 芽孢杆菌属和罗氏菌属等丰度提高 | [27,61] |
| 葡萄 Grape | db/db小鼠 | 肥胖 | 1% DM | 粪便和结肠菌群α多样性降低,阿克曼菌丰度提高,初级胆汁酸 合成相关菌——布劳特氏菌属和梭菌属丰度提高,次级胆汁酸代谢 合成菌——梭菌目、瘤胃球菌科和毛螺菌科丰度降低 | [44] |
| 葡萄籽 Grape seed | C57BL/6J小鼠 | DSS诱导肠炎 | 50 mg/kg BW | 上调DSS导致的F/B值降低,拟杆菌门、杜氏杆菌属和 韦荣氏球菌属丰度降低,疣微菌门和阿克曼菌属丰度提高 | [38,62] |
| 葡萄籽 Grape seed | C57BL/6J小鼠 | LPS诱导肠炎 | 250 mg/kg BW | 产生羟基类固醇脱氢酶(HSD)的毛螺菌科和瘤胃球菌科 丰度提高,粪便鹅脱氧胆酸(CDCA)和石胆酸(LCA)含量提高 | [61] |
| 葡萄籽 Grape seed | 断奶仔猪 | 饲养试验 | 250 mg/kg DM | F/B值降低,阿克曼菌、另枝菌和拟杆菌丰度提高, 粪便丙酸和丁酸含量提高 | [42] |
| 葡萄籽 Grape seed | 育肥猪 | 饲养试验 | 1% DM | 毛螺菌、梭菌、乳杆菌和瘤胃球菌丰度提高 | [53] |
| 葡萄籽 Grape seed | 生长猪 | 饲养试验 | 100、150和 200 mg/kg DM | 结肠菌群多样性下降, SCFAs生成菌丰度提高 | [63] |
| 葡萄籽 Grape seed | 爱拔益加肉鸡 | 饲养试验 | 200、 400 mg/kg DM | GSP标志菌群有乳杆菌纲、丙型变形菌纲、β变形菌纲、 Parasutterella和Erysipelatoclostridium丰度以及盲肠SCFAs (丁酸、丙酸和异丁酸)含量提高 | [64] |
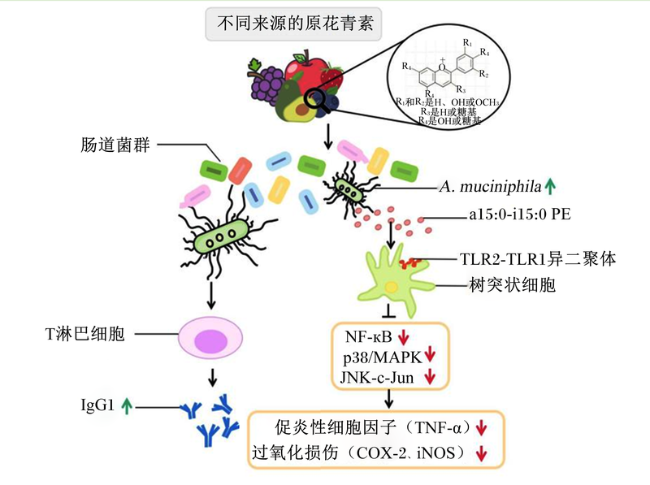
图2 PACs通过肠道嗜黏蛋白阿克曼菌调节免疫应答的作用机制(总结自文献[38-39,65⇓⇓-68])A. muciniphila:嗜黏蛋白阿克曼菌 Akkermansia muciniphila;a15:0-i15:0 PE:二酰基磷脂酰乙醇胺 1,2-dipalmitoyl-sn-glycero-3-phosphocholine;IgG1:免疫球蛋白G1 immunoglobulin G1;NF-кB:核因子-кB nuclear factor-kappa B;p38/MAPK:p38/丝裂原活化蛋白激酶 p38/mitogen-activated protein kinase;JNK-c-Jun:c-Jun氨基末端激酶-c-Jun c-Jun N-terminal kinase-c-Jun;TNF-α:肿瘤坏死因子-α tumor necrosis factor-α;COX-2:环氧化酶-2 cyclooxygenase-2;iNOS:诱导型一氧化氮合酶 inducible nitric oxide synthase。 Fig.2 Mechanism of PACs regulating intestinal immune responses through Akkermansia muciniphila (summary from the literature [38-39,65⇓⇓-68]) |
3.2 PACs通过肠道菌群代谢产物调节免疫应答
3.2.1 SCFAs-NOD样受体热蛋白结构域相关蛋白3(NOD-like receptor thermal protein domain associated protein 3,NLRP3)途径
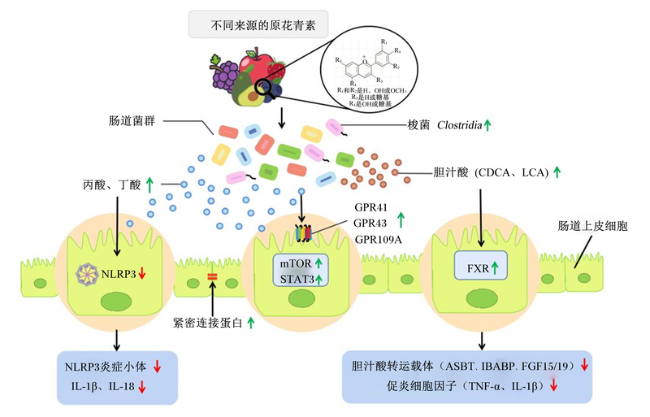


图3 PACs通过肠道菌群代谢产物调节免疫应答的作用机制(总结自文献[38,42,44,62,76-77,80])CDCA:鹅脱氧胆酸 chenodeoxycholic acid;LCA:石胆酸 lithocholic acid;GPR41:G蛋白偶联受体41 G protein-coupled receptor 41;GPR43:G蛋白偶联受体43 G protein-coupled receptor 43;GPR109A:G蛋白偶联受体109A G protein-coupled receptor 109A;mTOR:哺乳动物雷帕霉素靶蛋白 mammalian target of rapamycin;STAT3:信号转导与转录活化因子3 signal transducer and activator of transcription 3;NLRP3:NOD样受体蛋白3 NOD-like receptor protein 3;FXR:法尼醇X受体 Farnesoid X receptor;IL-1β:白细胞介素-1β interleukin-1β;IL-18:白细胞介素-18 interleukin-18;ASBT:顶端钠离子依赖性胆汁酸转运载体 apical sodium-dependent bile acid transporter;IBABP:回肠胆汁酸结合蛋白 ileal bile acid binding protein;FGF15/19:成纤维生长因子15/19 fibroblast growth factor 15/19;TNF-α:肿瘤坏死因子-α tumor necrosis factor-α。 Fig.3 Mechanism of PACs regulating intestinal immune responses through microbial metabolites (summary from the literature [38,42,44,62,76-77,80]) |