RESEARCH PAPER

Effects of Pueraria Polysaccharides on Serum Antioxidant and Immune Indexes and Gut Microbiota of Calves

  • LYU Shangkui , 1 ,
  • SHEN Yu 1, * ,
  • FAN Lei 1 ,
  • ZHANG Zeru 1 ,
  • ZHAO Yuquan 1 ,
  • YOU Liuchao 1 ,
  • ZHANG Yue 1, 2 ,
  • ZHANG Qiong 1 ,
  • SU Zhetong 2 ,
  • CAO Suizhong 1 ,
  • YU Shumin 1 ,
  • SHEN Liuhong , 1, **
Expand
  • 1 Medical Research Center for Cow Disease, Key Laboratory of Animal Disease and Human Health of Sichuan Province, College of Veterinary Medicine, Sichuan Agricultural University, Chengdu 611130, China
  • 2 Guangxi Innovate Medical Technology Co., Ltd., Lipu 546600, China
**associate professor, E-mail:

*Contributed equally

Received date: 2022-09-14

  Online published: 2023-03-16

Abstract

This experiment was conducted to investigate the effects of Pueraria polysaccharides on serum antioxidant and immune indexes and gut microbiota of calves. Twenty-four healthy (6.20±3.65) days of age Holstein calves with similar age body weight [(47.09±4.50) kg] were randomly divided into control group (group C) and test group (group T), each group contained 12 calves. Calves in group T were fed with 400 mg/kg Pueraria polysaccharides in the milk of each calve every day for 5 days, while others in group C were not added. The serum antioxidant indexes of superoxide dismutase (SOD), glutathione peroxidase (GSH-Px), nitric oxide synthase (NOS), catalase (CAT) activities and malondialdehyde (MDA) content, and immune indexes of CD4 molecules (CD4), immunoglobulin A (IgA), secretory immunoglobulin A (sIgA), immunoglobulin G (IgG) contents, the intestinally mucosal permeability index of diamine oxidase (DAO) activity, and the diversity and relative abundance of gut microbiota were detected on day 7. The results showed as follows: 1) compared with group C, the activities of SOD, CAT, NOS and GSH-Px in serum of calves of group T were increased by 10.16%, 1.79%, 7.05% and 3.43% (P>0.05), respectively, and the serum MDA content was decreased by 2.27% (P>0.05). 2) Compared with group C, the serum DAO activity of calves of group T was by 2.38% (P>0.05), and the contents of CD4, sIgA, IgA and IgG in serum were increased by 2.47%, 4.05%, 8.91% and 6.11% (P>0.05), respectively. 3) Compared with group C, the relative abundances of Bacteroidetes, Actinobacteria, Fusobacteria in gut of group T were increased, and the relative abundances of Firmicutes and Proteobacteria in gut were decreased. Compared with group C, the gut Bifidobacterium relative abundance of group T was significantly increased (P<0.05), the [Ruminococcus] gnavus group relative abundance was significantly decreased (P<0.05), and the Clostridium_sensu_stricto_1 relative abundance showed a down tendency (P=0.087). In conclusion, the Pueraria polysaccharides can improve the antioxidant capacity and immune function of calves, regulate the intestinal permeability, promote the growth of probiotics and inhibit proliferation of pathogen, so as to benefit the growth and development of calves.

Cite this article

LYU Shangkui , SHEN Yu , FAN Lei , ZHANG Zeru , ZHAO Yuquan , YOU Liuchao , ZHANG Yue , ZHANG Qiong , SU Zhetong , CAO Suizhong , YU Shumin , SHEN Liuhong . Effects of Pueraria Polysaccharides on Serum Antioxidant and Immune Indexes and Gut Microbiota of Calves[J]. Chinese Journal of Animal Nutrition, 2023 , 35(3) : 1696 -1704 . DOI: 10.12418/CJAN2023.160

肠道菌群对奶牛的整体生长性能和健康状况至关重要,特别是犊牛期,会由于各种因素(如腹泻、抗生素治疗或环境变化等)导致肠道菌群改变,影响其生长性能和抗病能力[1]。因此,维持犊牛健康的肠道菌群对预防其胃肠道疾病、提高饲料消化率及减少抗生素使用至关重要[2]。随着人们对抗生素耐药性和残留危害的认识,无抗、无残留、可增加动物免疫力和促进肠道健康发育的天然植物提取物的研究和开发,对促进奶牛养殖业无抗生产具有重要意义。多糖类、多酚类、皂苷类和氨基酸类等天然植物提取物可提高动物机体抵抗力[3-4]。植物多糖可有效提高动物机体抗氧化能力,增强免疫力,改善肠道健康,促进肠道发育,进而改善生长性能,已被广泛应用于动物生产[5-6]。研究发现,葛根主要成分为多糖、异黄酮和萜类等生物活性物质[7],具有增强免疫、抗氧化和抗菌等作用[7-8],可减轻各种原因引起的肠道病变和肠道菌群失衡,上调肠道有益菌水平,改善菌群结构,恢复肠道屏障功能[9-10]。本课题组前期研究发现,葛根多糖可通过调节犊牛二酰甘油、瓜氨酸、溶血磷脂酰胆碱18:0和胆绿素等血浆代谢物,从而减少犊牛腹泻率,促进其生长[11]。另外,血清二胺氧化酶(DAO)被临床用于作为评估各种动物肠黏膜通透性、完整性和黏膜屏障的标志物[12-14]。目前,葛根多糖对犊牛抗氧化、免疫、肠道黏膜通透性及肠道菌群的研究还未见报道。因此,结合葛根多糖的生物活性,在前期研究基础上,探究葛根多糖对犊牛血清抗氧化指标——超氧化物歧化酶(SOD)、丙二醛(MDA)、谷胱甘肽过氧化物酶(GSH-Px)、一氧化氮合酶(NOS)和过氧化氢酶(CAT),肠道黏膜通透性指标——DAO,血清免疫指标——CD4分子(CD4)、免疫球蛋白A(IgA)、分泌型免疫球蛋白A(sIgA)和免疫球蛋白G(IgG)及肠道菌群的影响,进一步为其在犊牛生产中的应用提供理论基础,为保护犊牛肠道健康提供天然无抗植物提取物。

1 材料与方法

1.1 试验材料

葛根多糖(纯度50.00%,平均分子质量1.09×10⁵ u)由广西某药物有限公司提供。

1.2 试验动物与试验设计

随机选取某规模化奶牛场半封闭统一饲舍、(6.20±3.65)日龄和体重[(47.09±4.50) kg]相近的新生健康荷斯坦犊牛24头,随机分为对照组(C组)和试验组(T组),每组12头。T组犊牛每头每天按每千克体重于牛奶中添加400 mg葛根多糖(添加剂量根据课题组前期试验结果[11],先溶于少量牛奶待犊牛吃完后,再饲喂剩余牛奶),连续添加5 d;C组犊牛无添加。所有试验犊牛均无既往病史和用药史。

1.3 饲养管理

按牧场犊牛常规饲养管理规定,定时饲喂,自由饮水,定期清理消毒。7日龄提供开食料,开食料营养水平见表1
表1 开食料营养水平(干物质基础)

Table 1 Nutrient levels of the starter (DM basis)%

项目 Items 含量 Content
水分 Moisture ≤12.5
粗脂肪 EE ≥2.0
粗灰分 Ash ≤9.0
总磷 TP ≥0.5
赖氨酸 Lys ≥0.6
粗蛋白质 CP ≥20.0
粗纤维 CF ≤8.0
钙 Ca 0.7~1.3
氯化钠 NaCl 0.3~0.7

1.4 指标测定

1.4.1 血清抗氧化、免疫指标及肠道黏膜通透性指标

试验第7天,分别采集C组和T组犊牛颈静脉血,离心后取血清,使用上海酶联试剂盒测定血清抗氧化指标:SOD(Cat.# SU-B77660)、MDA(Cat.# SU-B77036)、GSH-Px(Cat.# SU-B77736)、NOS(Cat.# SU-B77141)和CAT(Cat.# SU-B77735);血清免疫指标:CD4(Cat.# SU-B77596)、IgA(Cat.# SU-B77090)、sIgA(Cat.# SU-B77053)和IgG(Cat.# SU-B77091);肠道黏膜通透性指标:DAO(Cat.# SU-B77953)。

1.4.2 粪便菌群指标

试验第7天,采集C组和T组犊牛直肠深部粪便样品,放入液氮待测。使用NEB Next® UltraTMDNA Library Prep Kit试剂盒(Illumina,美国)构建文库,用特异性引物341F(5'-CCTACGGGNGGCWGCAG-3')和806R(5'-GGACTACHVGGGTWTCTAAT-3'),扩增16S rDNA的V3~V4区。文库质量通过Qubit@2.0荧光剂和Agilent生物分析仪2100系统评估。在Illumina MiSeq PE 2500平台测序并生成250 bp/300 bp双端读长。

1.5 数据统计分析

利用SPSS 26.0软件进行独立样本t检验,利用秩和检验分析粪便样品之间菌群相对丰度。结果以平均值和均值标准误(SEM)表示。P<0.05表示差异显著,0.05≤P<0.10表示有显著趋势。

2 结果

2.1 葛根多糖对犊牛血清抗氧化指标的影响

表2可知,与C组相比,T组犊牛血清SOD、CAT、NOS和GSH-Px活性分别提高了10.16%、1.79%、7.05%和3.43%(P>0.05),血清MDA含量降低了2.27%(P>0.05)。
表2 葛根多糖对犊牛血清抗氧化指标的影响

Table 2 Effects of Pueraria polysaccharides on serum antioxidant indexes of calves

项目
Items
组别 Groups SEM P
P-value
C T
超氧化物歧化酶 SOD/(U/mL) 28.14 31.00 4.14 0.629
丙二醛 MDA/(nmol/mL) 5.73 5.60 0.51 0.859
过氧化氢酶 CAT/(U/mL) 36.35 37.00 0.81 0.579
一氧化氮合酶 NOS/(U/mL) 64.50 69.05 8.35 0.714
谷胱甘肽过氧化物酶 GSH-Px/(U/mL) 264.35 273.41 6.49 0.348

2.2 葛根多糖对犊牛血清DAO活性和免疫指标的影响

表3可知,与C组相比,T组犊牛血清DAO活性降低了2.38%(P>0.05);血清CD4、sIgA、IgA和IgG含量分别提高了2.47%、4.05%、8.91%和6.11%(P>0.05),血清IgG含量呈现升高趋势(P=0.067)。
表3 葛根多糖对犊牛血清DAO活性和免疫指标的影响

Table 3 Effects of Pueraria polysaccharides on serum DAO activity and immune indexes of calves

项目
Items
组别 Groups SEM P
P-value
C T
二胺氧化酶 DAO/(U/mL) 0.42 0.41 0.04 0.851
CD4分子 CD4/(ng/mL) 12.53 12.84 0.45 0.640
分泌型免疫球蛋白A sIgA/(μg/mL) 25.42 26.45 0.65 0.348
免疫球蛋白A IgA/(μg/mL) 638.33 695.20 24.53 0.116
免疫球蛋白G IgG/(mg/mL) 2.29 2.43 0.05 0.067

2.3 葛根多糖对犊牛肠道菌群的影响

2.3.1 葛根多糖对犊牛肠道菌群α多样性的影响
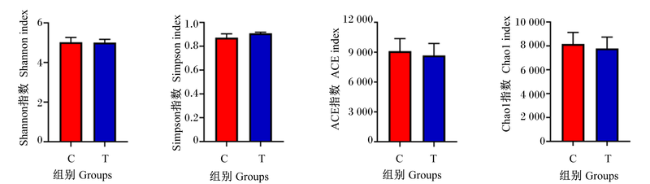
图1可知,与C组相比,T组犊牛肠道菌群α多样性指数,即Shannon指数、Simpson指数、ACE指数和Chao1指数均差异不显著(P>0.05)。
图1 葛根多糖对犊牛肠道菌群α多样性的影响

数据柱无字母表示差异不显著(P>0.05)。

Fig.1 Effects of Pueraria polysaccharides on gut microbiota α diversity of calves

Value columns with no letter mean no significant difference (P>0.05).

2.3.2 葛根多糖对犊牛肠道菌群组成的影响

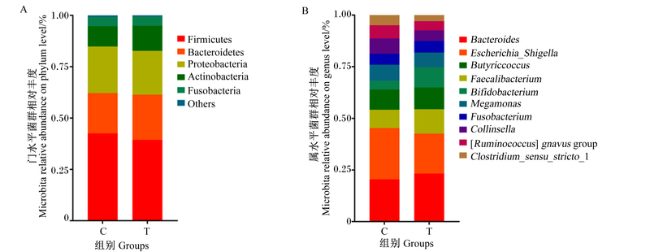
图2可知,在门水平上,C组肠道中优势菌门为厚壁菌门(Firmicutes,42.21%)、拟杆菌门(Bacteroidetes,19.44%)、变形杆菌门(Proteobacteria,22.51%)、放线菌门(Actinobacteria,9.78%)和梭杆菌门(Fusobacteria,4.40%)。与C组相比,T组肠道中拟杆菌门(24.48%)、放线菌门(14.67%)和梭杆菌门(4.49%)相对丰度增多,厚壁菌门(35.80%)和变形杆菌门(19.87%)相对丰度降低,且拟杆菌门/厚壁菌门比值增加。在属水平上,C组和T组肠道中优势菌属是拟杆菌属(Bacteroides)、埃希菌-志贺菌属(Escherichia_Shigella)、粪杆菌属(Faecalibacterium)、丁酸梭菌属(Butyricicoccus)、双歧杆菌属(Bifidobacterium)、巨单胞菌属(Megamonas)、梭杆菌属(Fusobacterium)、柯林斯菌属(Collinsella)、瘤胃球菌属([Ruminococcus] gnavus group)、狭义梭菌属1(Clostridium_sensu_stricto_1)。
图2 葛根多糖对犊牛肠道菌群组成的影响

Firmicutes:厚壁菌门;Bacteroidetes:拟杆菌门;Proteobacteria:变形杆菌门;Actinobacteria:放线菌门;Fusobacteria:梭杆菌门;Others:其他;Clostridium_sensu_stricto_1:狭义梭菌属1;[Ruminococcus] gnavus group:瘤胃球菌属;Collinsella:柯林斯菌属;Fusobacterium:梭杆菌属;Megamonas:巨单胞菌属;Bifidobacterium:双歧杆菌属;Butyriccoccus:丁酸梭菌属;Faecalibacterium:粪杆菌属;Escherichia_Shigella:埃希菌-志贺菌属;Bacteroides:拟杆菌属。下图同 the same as below。

Fig.2 Effects of Pueraria polysaccharides on gut microbiota composition of calves

表4可知,与C组相比,在属水平上,T组肠道中双歧杆菌属相对丰度显著增加(P<0.05),瘤胃球菌属相对丰度极显著降低(P<0.05),狭义梭菌属1相对丰度呈下降趋势(P=0.087)。
表4 葛根多糖对犊牛肠道菌群优势菌属相对丰度的影响

Table 4 Effects of Pueraria polysaccharides on relative abundances of dominant bacteria genus in gut microbiota of calves%

项目
Items
组别 Groups SEM P
P-value
C T
瘤胃球菌属 [Ruminococcus] gnavus group 5.28 16.12 0.73 0.008
双歧杆菌属 Bifidobacterium 3.54 12.32 2.16 0.033
狭义梭菌属1 Clostridium_sensu_stricto_1 4.10 0.41 1.04 0.087

2.3.3 葛根多糖对犊牛肠道菌群差异物种的影响

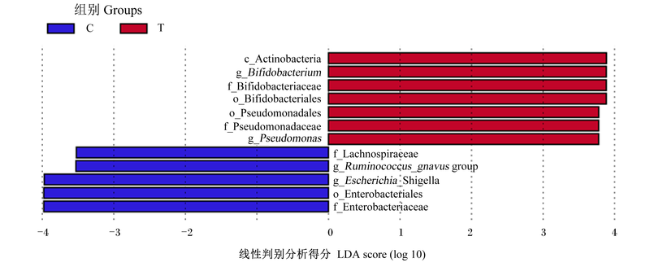
图3可知,使用线性判别分析(LDA)评估组间物种丰富度的差异,在LDA得分>3.5条件下,与C组相比,T组肠道中优势菌属为双歧杆菌属,而C组肠道中优势菌属为埃希菌-志贺菌属。
图3 犊牛肠道优势菌群差异物种分析

Pseudomonas:假单胞菌属;Lachnospiraceae:毛螺菌科;Enterobacteriaceae:肠杆菌科。

Fig.3 Analysis on different species of dominant microflora in gut of calves

3 讨论

3.1 葛根多糖对犊牛血清抗氧化指标的影响

动物内源性抗氧化指标主要包括SOD、GSH-Px、T-AOC和MDA等,可反映机体氧化应激和细胞损伤情况[15]。研究表明,葛根及其提取物具有良好的抗氧化、抗炎、抗应激、抗溃疡、保肝和调节免疫等作用[7-8];可显著降低活性氧(ROS)和MDA含量,同时增加SOD、CAT活性和谷胱甘肽(GSH)含量,降低脂质过氧化水平[16-17];可抑制氧化应激和细胞凋亡[18];可防止细胞内ROS介导的细胞凋亡和线粒体损伤[19];可改善C57Bl/6J小鼠体内SOD、GSH-Px活性和人T-AOC及MDA含量[9];可提高大鼠体内CAT、SOD和GSH-Px活性,增加核转录因子2(Nrf2)和血红素加氧酶-1(COX-1)基因和蛋白质表达,从而激活Nrf2介导信号通路,改善大鼠脂质积累和炎症水平[10];还可显著抑制脂多糖(LPS)诱导的NOSCOX-2基因表达,用于预防或治疗与炎症和氧化应激相关的疾病[20]。此外,葛根多糖体外也以剂量依赖式对1,1-二苯基-2-三硝基苯肼(DPPH)和羟基等自由基具有抗氧化活性[16]。本试验结果显示,葛根多糖可提高犊牛血清SOD、CAT、NOS和GSH-Px活性,虽差异不显著,但与葛根多糖可显著下调犊牛具有抗氧化调节的胆绿素水平和具有促炎作用的溶血磷脂酰胆碱18:0水平的前期研究结果[11]相互印证,可能由于本次试验饲喂葛根多糖时间较短,后续可适当延长饲喂时间,以提高葛根多糖对犊牛的抗氧化能力。

3.2 葛根多糖对犊牛血清DAO活性和免疫指标的影响

DAO是一种主要由肠黏膜细胞合成的高活性细胞内酶,参与细胞核酸和蛋白质合成,调控肠黏膜细胞增殖,其活性与肠黏膜通透性有关,通常用作哺乳动物肠道完整性、成熟性、通透性和黏膜屏障的标志物[12-14]。动物肠黏膜内源性DAO可防止腹泻和蠕动功能障碍等胃肠道不适,但在炎症性肠病和肠易激综合征等病理条件下,内源性DAO可丢失或失活[21]。另外,致病性大肠杆菌可导致新生犊牛血清DAO活性和LPS含量升高,导致肠通透性增加和肠屏障功能受损[22]。本试验中,葛根多糖可降低犊牛血清DAO活性,与其可促进犊牛具有肠道修复及发育作用的二酰甘油和瓜氨酸水平显著上调的前期研究结果[11]相互一致,表明葛根多糖可保护犊牛肠道通透性和肠屏障功能,可能是葛根提取物增强了肠上皮细胞增殖,并上调闭塞素表达而保护肠黏液屏障[23]。另外,CD4是一种糖蛋白,存在于辅助性T细胞、单核细胞、巨噬细胞和树突状细胞(DC细胞)表面,是哺乳动物辅助性T淋巴细胞主要的表面标志[24]。DC细胞的成熟(通过CD4、CD8和主要组织相容性复合物Ⅰ/Ⅱ表达增加体现)是启动免疫反应的关键因素,而葛根多糖可增加Toll样受体4(TLR4)下游的信号分子,诱导DC细胞功能成熟[25],还可显著提高sIgA、细胞因子和紧密连接蛋白等分泌水平,且显著增加肠系膜淋巴结T(CD4和CD8)细胞比例和杯状细胞数量,上调SOD活性,降低DAO活性和MDA含量,显著缓解环磷酰胺(CTX)诱导的小鼠体重减轻和肠道绒毛萎缩[26]。另外,葛根提取物可增加血清SOD、GSH-Px活性和免疫球蛋白(IgA、IgM和IgG)含量,从而增强肉牛免疫力和抗氧化能力[27]。本试验结果显示,葛根多糖同样可提高犊牛血清CD4、sIgA、IgA和IgG含量,虽差异不显著,但与上述文献结果趋势一致,也与葛根多糖可调节犊牛血液代谢、促进肠道发育、增强抗氧化能力、降低炎性反应,从而减少犊牛腹泻、促进犊牛生长的前期研究结果[11]相吻合,可能是葛根多糖提高了吞噬细胞的吞噬能力[28],从而对犊牛表现较好的免疫调节活性作用。

3.3 葛根多糖对犊牛肠道菌群的影响

哺乳动物肠道定植大量微生物,包括数万亿个细菌,这些细菌统称为肠道微生物群。微生物与宿主在共生关系中共同进化,除协助代谢外,还提供促进免疫稳态、免疫反应和防止病原体定植的多种功能[29],其变化可促进对致病菌的抵抗力或促进感染[30]。而幼龄动物肠道微生态不稳定,易引发各种肠道疾病[31]。因此,调节肠道菌群对增强其机体抵抗力、促进其生长具有积极作用。而多糖可作为肠道菌群重要能量来源而被菌群发酵降解,产生包括短链脂肪酸在内的代谢物,可促进肠道健康[32-33]。本研究结果显示,新生犊牛肠道厚壁菌门和拟杆菌门最丰富,与文献报道[34]一致;厚壁菌门与碳水化合物和蛋白质的吸收有关,拟杆菌门在非纤维物质的降解中发挥重要作用[35]。葛根提取物可增加机体抗氧化能力,显著增加乳酸杆菌和拟杆菌等有益菌相对丰度,降低有害菌相对丰度[9-10]。本试验中,葛根多糖降低了犊牛肠道厚壁菌门相对丰度,提高了拟杆菌门相对丰度,且增加了拟杆菌门/厚壁菌门比值。拟杆菌门/厚壁菌门比值降低易导致肠易激综合征的发生[36],本试验结果与之相反,表明葛根多糖可预防犊牛肠道不适。另外,变形杆菌相对丰度是哺乳动物肠上皮功能障碍潜在诊断微生物特征[37],与肠炎、免疫失衡和菌群失调密切相关,被用作衡量肠道健康的重要指标[38]。葛根提取物可通过显著降低变形杆菌相对丰度,调节肠道微生物群的平衡[39]。本试验中,葛根多糖降低了犊牛肠道变形杆菌相对丰度,与上述结果一致。这表明葛根多糖抑制了犊牛肠道致病菌繁殖,可减少犊牛腹泻,从而利于犊牛生长发育。
肠道菌群影响机体免疫力的一个重要机制是通过发酵产生短链脂肪酸从而改善宿主健康[40]。短链脂肪酸是肠道上皮细胞主要能量来源,并可提高肠道完整性,且具有免疫调节作用[41]。双歧杆菌是产生短链脂肪酸的主要菌属,是健康菌群组成之一[42],可通过促进CD4 T细胞-树突细胞相互作用和淋巴细胞增殖而提高肠道黏膜免疫[29]。葛根提取物可特异性增加乳酸杆菌和双歧杆菌等相对丰度[43],且可显著降低肠道异戊酸浓度,增加有益细菌相对丰度,缓解抗生素性腹泻小鼠肠道病变和微生物群失调[4]。此外,双歧杆菌通过定植抗性作用,抑制宿主自身肠道的潜在病原菌——大肠杆菌和肠杆菌科等[44]。本试验发现,在属水平上,葛根多糖可显著增加犊牛肠道双歧杆菌属相对丰度,极显著降低瘤胃球菌属相对丰度,且狭义梭菌属1相对丰度呈下降趋势。新生犊牛瘤胃球菌属相对丰度增加可导致腹泻[45]。这说明葛根多糖具有预防犊牛腹泻的作用,印证了葛根多糖可减少犊牛腹泻率的临床试验结果[11],综上所述,葛根多糖可作为预防犊牛腹泻和促进犊牛健康生长的饲料添加剂。

4 结论

葛根多糖可提高犊牛抗氧化能力,增强免疫功能,调节肠道通透性,促进肠道有益菌生长,抑制有害菌增殖,从而有利于犊牛的生长发育。
[1]
KIM E T, LEE S J, KIM T Y, et al. Dynamic changes in fecal microbial communities of neonatal dairy calves by aging and diarrhea[J]. Animals, 2021, 11(4):1113.

DOI

[2]
FAN P X, KIM M, LIU G, et al. The gut microbiota of newborn calves and influence of potential probiotics on reducing diarrheic disease by inhibition of pathogen colonization[J]. Frontiers in Microbiology, 2021, 12:772863.

[3]
李欣, 童津津, 赵佳桢, 等. 氧化应激、炎症和免疫失衡三方联动效应与奶牛常见健康问题的联系及使用植物提取物进行干预的研究进展[J]. 动物营养学报, 2021, 33(12):6666-6675.

DOI

LI X, TONG J J, ZHAO J Z, et al. Relationship between oxidative stress,inflammation and immune imbalance in tripartite linkage effect and common health problems of dairy cows and research progress of intervention with plant extracts[J]. Chinese Journal of Animal Nutrition, 2021, 33(12):6666-6675. (in Chinese)

[4]
CHEN R, LIU B, WANG X Y, et al. Effects of polysaccharide from Pueraria lobata on gut microbiota in mice[J]. International Journal of Biological Macromolecules, 2020, 158:740-749.

DOI

[5]
董金金, 高艳霞, 李妍, 等. 酵母多糖对哺乳犊牛胃肠道发育及消化酶活性的影响[J]. 动物营养学报, 2018, 30(12):5247-5254.

DONG J J, GAO Y X, LI Y, et al. Effects of yeast polysaccharide on gastrointestinal development and digestive enzyme activity of sucking calves[J]. Chinese Journal of Animal Nutrition, 2018, 30(12):5247-5254. (in Chinese)

[6]
ZHU W, ZHOU S X, LIU J H, et al. Prebiotic,immuno-stimulating and gut microbiota-modulating effects of Lycium barbarum polysaccharide[J]. Biomedicine & Pharmacotherapy, 2020, 121:109591.

[7]
ZHU W F, LI J L, MENG X W, et al. [Research advances in chemical constituents and pharmacological activities of Pueraria genus][J]. China Journal of Chinese Materia Medica, 2021, 46(6):1311-1331.

[8]
BHARTI R, CHOPRA B S, RAUT S, et al. Pueraria tuberosa:a review on traditional uses,pharmacology,and phytochemistry[J]. Frontiers in Pharmacology, 2020, 11:582506.

[9]
XU X, GUO Y, CHEN S Q, et al. The positive influence of polyphenols extracted from Pueraria lobata root on the gut microbiota and its antioxidant capability[J]. Frontiers in Nutrition, 2022, 9:868188.

[10]
ZHAO W J, PENG D, LI W J, et al. Probiotic-fermented Pueraria lobata (Willd.) Ohwi alleviates alcoholic liver injury by enhancing antioxidant defense and modulating gut microbiota[J/OL]. Journal of the Science of Food and Agriculture: [2022---08-15]. https://pubmed.ncbi.nlm.nih.gov/35655427/DOI:10.1002/jsfa.12049.

DOI

[11]
莘余, 吕尚揆, 尤留超, 等. 葛根多糖对健康犊牛基础临床,生理生化指标及血浆代谢物的影响[J]. 动物营养学报, 2022, 34(10):6609-6619.

DOI

SHEN Y, LV S K, YOU L C, et al. Effects of Pueraria polysaccharides on basic clinical indexes,physiological and biochemical indexes and plasma metabolites of healthy calves[J]. Chinese Journal of Animal Nutrition, 2022, 34(10):6609-6619. (in Chinese)

DOI

[12]
CAI J R, CHEN H, WENG M L, et al. Diagnostic and clinical significance of serum levels of D-lactate and diamine oxidase in patients with Crohn's disease[J]. Gastroenterology Research and Practice, 2019, 2019:8536952.

[13]
FUKUDOME I, KOBAYASHI M, DABANAKA K, et al. Diamine oxidase as a marker of intestinal mucosal injury and the effect of soluble dietary fiber on gastrointestinal tract toxicity after intravenous 5-fluorouracil treatment in rats[J]. Medical Molecular Morphology, 2014, 47(2):100-107.

DOI PMID

[14]
DIERYCK I, DE BACKERE J, PAESHUYSE J. Effect of hatching system and prophylactic antibiotic use on serum levels of intestinal health biomarker diamine oxidase in broilers at an early age[J]. Animal, 2022, 16(4):100493.

[15]
DUANGJAN C, RANGSINTH P, ZHANG S X, et al. Vitis vinifera leaf extract protects against glutamate-induced oxidative toxicity in HT22 hippocampal neuronal cells and increases stress resistance properties in Caenorhabditis elegans[J]. Frontiers in Nutrition, 2021, 8:634100.

[16]
SHAO X Y, HE T, LAI Y L, et al. Water-soluble polysaccharides extracted from Pueraria lobata delay aging of Caenorhabditis elegans under heat stress[J]. Plant Foods for Human Nutrition, 2022, 77(2):220-225.

DOI

[17]
JEARAPONG N, CHATUPHONPRASERT W, JARUKAMJORN K. Miroestrol,a phytoestrogen from Pueraria mirifica,improves the antioxidation state in the livers and uteri of β-naphthoflavone-treated mice[J]. Journal of Natural Medicines, 2014, 68(1):173-180.

DOI

[18]
SHUKLA R, BANERJEE S, TRIPATHI Y B. Antioxidant and antiapoptotic effect of aqueous extract of Pueraria tuberosa (Roxb. Ex willd.) DC. on streptozotocin-induced diabetic nephropathy in rats[J]. BMC Complementary and Alternative Medicine, 2018, 18(1):156.

DOI

[19]
GAO Y, WANG X, HE C N. An isoflavonoid-enriched extract from Pueraria lobata (kudzu) root protects human umbilical vein endothelial cells against oxidative stress induced apoptosis[J]. Journal of Ethnopharmacology, 2016, 193:524-530.

DOI

[20]
SON E, YOON J M, AN B J, et al. Comparison among activities and isoflavonoids from Pueraria thunbergiana aerial parts and root[J]. Molecules, 2019, 24(5):912.

DOI

[21]
NEREE A T, SORET R, MARCOCCI L, et al. Vegetal diamine oxidase alleviates histamine-induced contraction of colonic muscles[J]. Scientific Reports, 2020, 10(1):21563.

DOI PMID

[22]
HE L N, WANG C J, SIMUJIDE H, et al. Effect of early pathogenic Escherichia coli infection on the intestinal barrier and immune function in newborn calves[J]. Frontiers in Cellular and Infection Microbiology, 2022, 12:818276.

[23]
WANG Q S, WANG Y L, ZHANG W Y, et al. Puerarin from Pueraria lobata alleviates the symptoms of irritable bowel syndrome-diarrhea[J]. Food & Function, 2021, 12(5):2211-2224.

[24]
KATO-MORI Y, OKAMURA T, KAWASHITA N, et al. Characterization of a variant CD4 molecule in Japanese Black cattle[J]. Veterinary Immunology and Immunopathology, 2021, 232:110167.

[25]
KIM H S, SHIN B R, LEE H K, et al. A polysaccharide isolated from Pueraria lobata enhances maturation of murine dendritic cells[J]. International Journal of Biological Macromolecules, 2013, 52:184-191.

DOI

[26]
CAI G F, WU C H, MAO N N, et al. Isolation,purification and characterization of Pueraria lobata polysaccharide and its effects on intestinal function in cyclophosphamide-treated mice[J]. International Journal of Biological Macromolecules, 2022, 218:356-367.

DOI

[27]
PENG T, SHANG H L, YANG M R, et al. Puerarin improved growth performance and postmortem meat quality by regulating lipid metabolism of cattle under hot environment[J]. Animal Science Journal, 2021, 92(1):e13543.

[28]
DONG Z, ZHANG M M, LI H X, et al. Structural characterization and immunomodulatory activity of a novel polysaccharide from Pueraria lobata (Willd.) Ohwi root[J]. International Journal of Biological Macromolecules, 2020, 154:1556-1564.

DOI

[29]
PICKARD J M, ZENG M Y, CARUSO R, et al. Gut microbiota:role in pathogen colonization,immune responses,and inflammatory disease[J]. Immunological Reviews, 2017, 279(1):70-89.

DOI

[30]
BÄUMLER A J, SPERANDIO V. Interactions between the microbiota and pathogenic bacteria in the gut[J]. Nature, 2016, 535(7610):85-93.

DOI

[31]
VOGT S L, FINLAY B B. Gut microbiota-mediated protection against diarrheal infections[J]. Journal of Travel Medicine, 2017,24 (Suppl.1):S39-S43.

[32]
FANG Q Y, HU J L, NIE Q X, et al. Effects of polysaccharides on glycometabolism based on gut microbiota alteration[J]. Trends in Food Science & Technology, 2019, 92:65-70.

[33]
LI L F, YAO H, LI X J, et al. Destiny of Dendrobium officinale polysaccharide after oral administration:indigestible and nonabsorbing,ends in modulating gut microbiota[J]. Journal of Agricultural and Food Chemistry, 2019, 67(21):5968-5977.

DOI

[34]
HENNESSY M, INDUGU N, VECCHIARELLI B, et al. Short communication:comparison of the fecal bacterial communities in diarrheic and nondiarrheic dairy calves from multiple farms in southeastern Pennsylvania[J]. Journal of Dairy Science, 2021, 104(6):7225-7232.

DOI

[35]
GRUNINGER R J, SENSEN C W, MCALLISTER T A, et al. Diversity of rumen bacteria in Canadian cervids[J]. PLoS One, 2014, 9(2):e89682.

[36]
RODIÑO-JANEIRO B K, VICARIO M, ALONSO-COTONER C, et al. A review of microbiota and irritable bowel syndrome:future in therapies[J]. Advances in Therapy, 2018, 35(3):289-310.

DOI

[37]
LITVAK Y, BYNDLOSS M X, TSOLIS R M, et al. Dysbiotic Proteobacteria expansion:a microbial signature of epithelial dysfunction[J]. Current Opinion in Microbiology, 2017, 39:1-6.

DOI

[38]
SHIN N R, WHON T W, BAE J W. Proteobacteria:microbial signature of dysbiosis in gut microbiota[J]. Trends in Biotechnology, 2015, 33(9):496-503.

DOI

[39]
QIN Y H. Pueraria lobata targeted preparation improves the clinical symptoms of cervical spondylosis by regulating the balance of gut microbiota[J]. Computational and Mathematical Methods in Medicine, 2022, 2022:2136807.

[40]
SHAO J, LI Z C, GAO Y P, et al. Construction of a“bacteria-metabolites”co-expression network to clarify the anti-ulcerative colitis effect of flavonoids of Sophora flavescens aiton by regulating the“host-microbe”interaction[J]. Frontiers in Pharmacology, 2021, 12:710052.

[41]
DO PRADO S B R, MINGUZZI B T, HOFFMANN C, et al. Modulation of human gut microbiota by dietary fibers from unripe and ripe papayas:distinct polysaccharide degradation using a colonic in vitro fermentation model[J]. Food Chemistry, 2021, 348:129071.

[42]
GÓMEZ B, GULLÓN B, REMOROZA C, et al. Purification,characterization,and prebiotic properties of pectic oligosaccharides from orange peel wastes[J]. Journal of Agricultural and Food Chemistry, 2014, 62(40):9769-9782.

DOI

[43]
YANG Y F, LI M X, WANG Q, et al. Pueraria lobata starch regulates gut microbiota and alleviates high-fat high-cholesterol diet induced non-alcoholic fatty liver disease in mice[J]. Food Research International, 2022, 157:111401.

[44]
VAN VLIET M J, TISSING W J E, DUN C A J, et al. Chemotherapy treatment in pediatric patients with acute myeloid leukemia receiving antimicrobial prophylaxis leads to a relative increase of colonization with potentially pathogenic bacteria in the gut[J]. Clinical Infectious Diseases, 2009, 49(2):262-270.

DOI PMID

[45]
REDDING L E, BERRY A S, INDUGU N, et al. Gut microbiota features associated with Clostridioides difficile colonization in dairy calves[J]. PLoS One, 2021, 16(12):e0251999.

Outlines

/