RESEARCH PAPER

Effects of Fucoidan on Rumen Microflora and Metabolomics of Weaned Lambs

  • WANG Shengnan ,
  • YANG Weiguang ,
  • YIN Fuquan , *
Expand
  • College of Coastal Agricultural Sciences, Guangdong Ocean University, Zhanjiang 524088, China
*professor, E-mail:

Received date: 2022-07-19

  Online published: 2023-03-16

Abstract

This experiment was conducted to investigate the effects of fucoidan on rumen microflora and metabolomics of weaned lambs. Sixty healthy 60-day-old weaned lambs (Chuanzhong black goat) with similar body weight of (12.5±0.5) kg were randomly divided into 4 groups with 15 lambs in each group. Lambs in control group (CON group) were fed a basal diet, and others in experimental groups were fed the basal diet supplemented with 0.1% (F1 group), 0.3% (F2 group) and 0.5% (F3 group) fucoidan, respectively. The re-experimental period lasted for 7 days, and the experimental period lasted for 30 days. The results showed as follows: 1) compared with the CON group, the final weight, average daily gain and average daily feed intake of F2 and F3 groups were significantly increased (P<0.05), and the feed to gain ratio of F1, F2 and F3 groups was significantly decreased (P<0.05). 2) Compared with the CON group, the rumen pH and of acetic acid, butyric acid and isobutyric acid contents and acetic acid/propionic acid of F1, F2 and F3 groups were significantly increased (P<0.05), and the rumen propionic acid content of F2 and F3 groups was significantly increased (P<0.05). 3) At phyla levels, compared with the CON group, the rumen Verrucomicrobia relative abundance of F1, F2 and F3 groups was significantly increased (P<0.05); the rumen Bacteroidetes relative abundance of F1 and F3 groups was significantly increased (P<0.05), and the Actinobacteria, Euryarchaeota and Spirochaetes relative abundances were significantly decreased (P<0.05). At genera levels, compared with the CON group, the relative abundances of unspecified_BS11, unspecified_RF16 and unspecified_S24_7 in rumen of F1 and F3 groups were significantly increased (P<0.05), and the unspecified_Lachnospiraceaea and unspecified_Veillonellaceae were significantly decreased (P<0.05). 4) The metabolomics results showed that in the positive ion mode, compared with the CON group, the rumen metabolite contents of carbohydrates, peptides, nucleic acids and hormones and transmitters of F1, F2 and F3 groups were significantly decreased (P<0.05), and the metabolite contents of organic acids, vitamins and cofactors, steroids and lipids were significantly increased (P<0.05). In the negative ion mode, compared with the CON group, the rumen metabolite contents of steroids and hormones and transmitters of F1, F2 and F3 groups were significantly decreased (P<0.05), and other metabolite contents were significantly increased (P<0.05). It is concluded that the fucoidan can improve the rumen fermentation and rumen microbial flora diversity and relative abundance of weaned lambs, and affect the rumen metabolites and metabolic pathways.

Cite this article

WANG Shengnan , YANG Weiguang , YIN Fuquan . Effects of Fucoidan on Rumen Microflora and Metabolomics of Weaned Lambs[J]. Chinese Journal of Animal Nutrition, 2023 , 35(3) : 1827 -1840 . DOI: 10.12418/CJAN2023.172

断奶是羔羊生长的关键阶段,由于母幼分离以及饲粮和饲养环境的改变,对羔羊生长、胃肠道发育等带来负面影响[1-2]。通过添加抗生素可以降低羔羊因断奶产生的应激反应,但是,使用抗生素也会出现严重的后遗症。随着我国实施全面禁抗政策,寻找抗生素的替代物对减弱断奶羔羊的应激反应,提高羔羊生长及胃肠道发育具有重要意义。岩藻多糖是来自海藻的天然海洋植物提取物,其被证实具有多种生物学功能,并应用于人类保健以及小鼠、仔猪等动物生产中,但其在反刍动物营养调控中的应用则鲜有报道。
岩藻多糖作为可溶性膳食纤维,能够起到维持消化道菌群稳态、促进胃肠道发育的作用,进而提高断奶后羔羊的生长性能。瘤胃是反刍动物消化吸收的重要部位,瘤胃微生物将饲粮分解成小分子的有机物与短链脂肪酸,由瘤胃上皮细胞吸收后为反刍动物提供营养和能量[3-6]。因此,可以通过饲粮营养水平来调控瘤胃微生物结构。Quijada等[7]在羔羊饲粮中添加来自甜菜和大蒜的低聚果糖,通过16S rRNA测序发现,与对照组相比,低聚果糖显著提高了瘤胃中双歧杆菌、罗伊氏乳杆菌和韦荣氏球菌的相对丰度,这3种有益菌对瘤胃核心菌群定植、免疫系统和生长性能有重要意义。目前研究多集中于功能性多糖,并无藻源多糖应用于反刍动物中的报道。因此,本试验旨在研究岩藻多糖对断奶羔羊瘤胃微生物区系及代谢组学的影响,以期为藻源多糖应用于反刍动物生产提供理论依据。

1 材料与方法

1.1 试验材料

岩藻多糖是由某公司提供,纯度为98%,其中硫酸盐离子含量为28.9%。岩藻多糖为含有以岩藻糖为主和多种单糖残基以及硫酸基的水溶性多糖,主要成分除岩藻糖和硫酸酯外,还含有其他单糖(甘露糖、半乳糖、葡萄糖等)和糖醛酸,有些还具有乙酰基和蛋白质。

1.2 试验设计

选用60只60日龄平均体重为(12.5±0.5) kg的断奶去势公羔羊(川中黑山羊),随机分为4组,每组15只,每3只在同一栏中。对照组(CON组)饲喂基础饲粮,试验组在基础饲粮中分别添加0.1%(F1组)、0.3%(F2组)和0.5%(F3组)的岩藻多糖。基础饲粮组成及营养水平见表1。预试期7 d,正试期30 d。每天08:30和17:30各饲喂1次,自由饮水。
表1 基础饲粮组成及营养水平(干物质基础)

Table 1 Composition and nutrient levels of the basal diet (DM basis)%

项目 Items 含量 Content
原料 Ingredients
象草 Pennisetum purpureum 35.00
玉米 Corn 40.89
豆粕 Soybean meal 13.98
麸皮 Wheat bran 7.15
食盐 NaCl 0.65
磷酸氢钙 CaHPO4 0.84
石粉 Limestone 0.84
预混料 Premix1) 0.65
合计 Total 100.00
营养水平 Nutrient levels2)
干物质 Dry matte 88.86
代谢能 Metabolic energy/(MJ/kg) 10.43
粗蛋白质 Crude protein 12.06
中性洗涤纤维 Neutral detergent fiber 30.06
酸性洗涤纤维 Acid detergent fiber 16.39
钙 Calcium 0.76
磷 Phosphorus 0.54

1)预混料为每千克饲粮提供 The premix provided the following per kg of the diet: VA 8 000 IU,VD 2 000 IU,VE 40 IU,Cu 12 mg,Fe 70 mg,Mn 50 mg,Zn 80 mg,I 1.0 mg,Se 0.27 mg,Co 0.3 mg。

2)代谢能为计算值,其他为实测值。Metabolic energy was a calculated value, while the others were measured values.

1.3 样品采集和指标检测

1.3.1 样品的采集与制备

在正式试验的第1天和第30天晨饲前对每只羔羊进行称重并记录。每天记录精料和粗料的采食量,计算平均日增重(ADG)、平均日采食量(ADFI)和料重比(F/G)。
饲养结束后每组挑选6只羔羊进行屠宰,屠宰前禁食12 h,瘤胃液用4层纱布过滤后于-80 ℃保存,用于后续微生物区系及代谢组学分析。

1.3.2 瘤胃液总菌DNA提取及Illumina Novaseq测序与分析

瘤胃内容物样本的基因组总DNA提取采用溴代十六烷基三甲胺血红蛋白(CTAB)测定法,之后用1%的琼脂糖凝胶电泳检测总DNA的质量和浓度,最后使用无菌水将总DNA样本稀释为1 ng/μL。使用特异性引物341F(5'-CCTAYGGRBGCASCAG-3')和806R(5'-GGACTACNNGGGTATCTAAT-3')对V3+V4可变区进行聚合酶链式反应(PCR)。PCR扩增反应程序为:98 ℃预变性1 min;30个循环(98 ℃,10 s;50 ℃,30 s;72 ℃,30 s);72 ℃,5 min。之后使用2%琼脂糖凝胶电泳纯化PCR产物。最后使用凝胶回收试剂盒(Qiagen,德国)回收纯化PCR产物。
使用建库试剂盒(Illumina,美国)进行文库构建,构建好的文库用Qubit核酸蛋白定量仪(Thermo Scientific,美国)进行质量评估。然后,在Illumina NovaSeq平台上对文库进行测序,产生250 bp的成对末端读数。
使用QIIME2 data2对原始数据进行质控、修剪、去噪和拼接,然后用QIIME2 feature-classifier将扩增子序列变异(ASV)的代表序列与预先设置好的13.8版本99%相似度的Greengens基因数据库进行比对,得到微生物物种的分类信息表。使用ANOVA方法鉴定组间相对丰度有差异的细菌。多样性指数用QIIME2 core-diversity插件计算,Alpha多样性指数包括Chao1、Shannon和Simpson指数。用主成分分析(PCoA)图表示组间的Beta多样性。用PICTRUSt软件对微生物的功能组成进行预测。

1.3.3 瘤胃液中pH及挥发性脂肪酸含量的检测

使用便携式pH测定计(S220-K型)检测瘤胃液的pH,瘤胃液挥发性脂肪酸含量采用Trace 1310气相色谱仪检测。

1.3.4 瘤胃液代谢组学分析

1)取100 μL瘤胃液样本置于EP管中,加入400 μL 80%的甲醇溶液;2)漩涡振荡,冰浴静置5 min,之后15 000×g,4 ℃离心20 min;3)取上清液加质谱级水稀释至甲醇含量为53%;4)15 000×g,4 ℃离心20 min,取上清,进行液相色谱质谱联(LC-MS)分析。
使用Vanquish UHPLC超高效液相色谱仪(Thermo Fisher,美国)和Q ExactiveTM HF质谱仪(Thermo Fisher,美国)。色谱条件为:正模式下,流动相A为0.1%的甲酸,流动相B为甲醇溶液;负模式下,流动相A为5 mmol/L醋酸铵(pH 9.0),流动相B为甲醇溶液。色谱柱HypesilGoldcolumn(C18),柱温为40 ℃,流速为0.2 mL/min。色谱梯度洗脱程序如表2。质谱条件为:扫描范围选择质荷比(m/z) 100~1 500;电喷雾离子化(ESI)源的设置如下:喷涂电压:3.2 kV;鞘气流量:40 arb;辅助气流量:10 arb;毛细管温度:320 ℃;极性:正,否定;MS/MS data相关扫描。
表2 色谱梯度洗脱程序

Table 2 Chromatographic conditions for gradient elution%

时间
Time/min
流动相A
Mobile phase A
流动相B
Mobile phase B
0 98 2
1.5 98 2
12.0 0 85
14.0 0 100
14.1 98 2
17.0 98 2

1.4 数据统计与分析

将下机的原始数据导入Compound Discoverer 3.1软件中,进行每个代谢物的峰对齐、峰识别、保留时间矫正、代谢物峰面积定量等操作。之后将信息与数据库进行比对,获得代谢物的详细信息。使用KEGG、HMDB等数据库对代谢物进行注释,之后通过软件包对数据进行多元统计分析,统计分析操作均在微科盟生物检测平台操作执行。试验数据采用Excel 2019进行初步汇总和整理,采用SPSS 26.0软件中的ANOVA过程进行单因素方差分析,用Duncan氏法进行多重比较。数据以平均值和均值标准误(SEM)表示,P<0.05表示差异显著。

2 结果

2.1 岩藻多糖对断奶羔羊生长性能的影响

表3可知,各组之间羔羊初重无显著差异(P>0.05)。与CON组相比,F2、F3组的末重显著升高(P<0.05),F1、F2、F3组的F/G显著降低(P<0.05),F2和F3组的ADG和ADFI显著升高(P<0.05)。
表3 岩藻多糖对断奶羔羊生长性能的影响

Table 3 Effects of fucoidan on growth performance of weaned lambs

项目
Items
组别 Groups SEM P
P-value
CON F1 F2 F3
初重 IBW/kg 12.20 11.38 12.27 12.97 0.99 0.25
末重 FBW/kg 12.85a 12.88a 15.28b 15.12b 1.09 0.02
平均日增重ADG/(g/d) 45.00c 50.06c 100.33a 72.01b 9.71 <0.01
平均日采食量ADFI/(g/d) 501.09b 525.09b 597.01a 565.02a 22.71 0.01
料重比 F/G 11.25a 10.60b 6.05c 8.25c 1.08 0.01

同行数据肩标不同小写字母表示差异显著(P<0.05),相同或无字母表示差异不显著(P>0.05)。下表同。

In the same row, values with different small letter superscripts mean significant difference (P<0.05), while with the same or no letter superscripts mean no significant difference (P>0.05). The same as below.

2.2 岩藻多糖对断奶羔羊瘤胃pH和挥发性脂肪酸含量的影响

表4可知,与CON组相比,F1、F2、F3组的瘤胃pH和乙酸、丁酸、异丁酸含量及乙酸/丙酸显著升高(P<0.05),F2、F3组的瘤胃丙酸含量显著升高(P<0.05)。
表4 岩藻多糖对断奶羔羊瘤胃液pH和挥发性脂肪酸含量的影响

Table 4 Effects of fucoidan on rumen pH and volatile fatty acid contents of weaned lambs

项目
Items
组别 Groups SEM P
P-value
CON F1 F2 F3
pH 6.63b 6.89a 6.85a 6.86a 0.05 0.04
乙酸 Acetic acid/(mmol/L) 43.16d 50.42c 60.06b 61.07a 8.16 <0.01
丙酸 Propionic acid/(mmol/L) 14.53c 14.53c 14.83b 18.28a 1.36 <0.01
丁酸 Butyric acid/(mmol/L) 12.13d 12.26c 12.37b 13.29a 0.82 <0.01
异丁酸 Isobutyric acid/(mmol/L) 0.23d 0.27c 0.34b 0.45a 0.30 <0.01
乙酸/丙酸 Acetic acid/propionic acid 2.97d 3.47b 4.05a 3.34c 0.04 <0.01

2.3 岩藻多糖对断奶羔羊瘤胃菌群丰富度和多样性的影响

表5可知,各组之间瘤胃菌群丰富度指数Chao1、Faith指数、观测物种数和多样性指数Shannon、Simpson指数均无显著差异(P>0.05)。
表5 瘤胃菌群丰富度和多样性指数

Table 5 Rumen flora richness and diversity index

项目
Items
组别 Groups SEM P
P-value
CON F1 F2 F3
观测物种数 Observed-species 1 454.00 1 381.33 1 330.67 1 243.00 129.12 0.46
Chao1指数 Chao1 index 1 472.71 1 401.78 1 344.63 1 254.19 129.33 0.43
Faith指数 Faith index 84.81 75.68 86.34 71.35 8.54 0.31
Shannon指数 Shannon index 8.97 8.61 8.66 8.64 0.37 0.75
Simpson指数 Simpson index 0.99 0.99 0.98 0.99 0.01 0.68
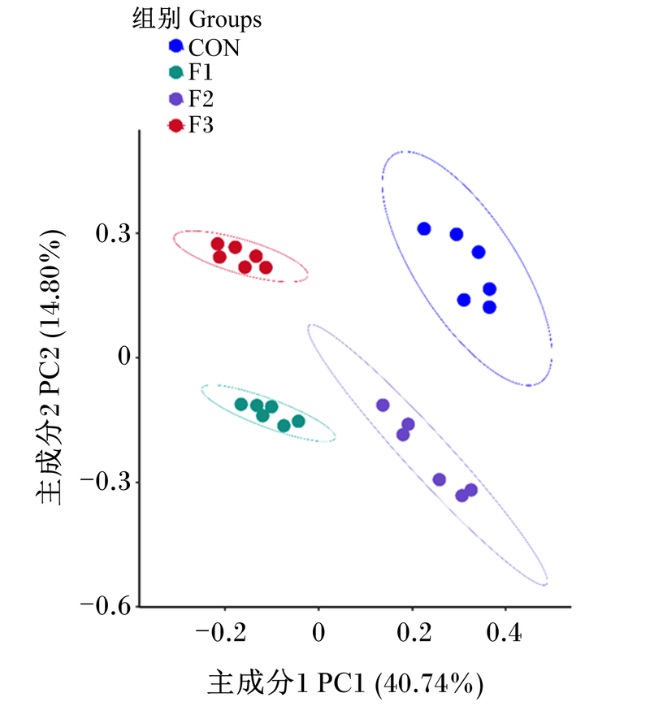
图1可知,各样本区分明显,瘤胃菌群明显分开。
图1 瘤胃菌群主成分分析图

Fig.1 PCoA diagram of rumen flora

2.4 岩藻多糖对断奶羔羊瘤胃微生物门、属水平相对丰度的影响

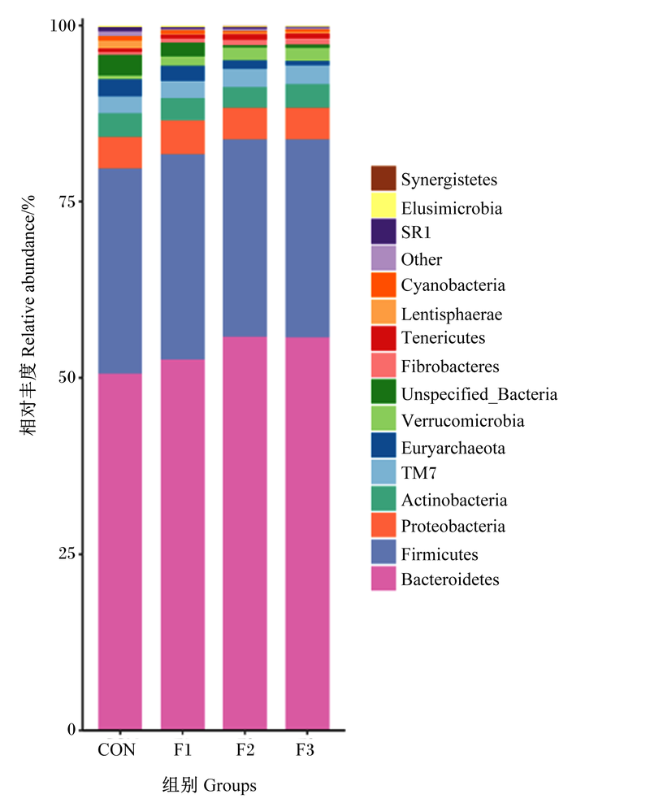
图2可知,断奶羔羊的瘤胃中厚壁菌门(Firmicutes)和拟杆菌门(Bacteroidetes)为优势菌门,占总相对丰度的70%以上。由表6可知,与CON组相比,F1、F2、F3组的瘤胃中疣微菌门(Verrucomicrobia)的相对丰度显著升高(P<0.05);F1、F3组的瘤胃中Bacteroidetes的相对丰度显著升高(P<0.05),放线菌门(Actinobacteria)、广古菌门(Euryarchaeota)、螺旋菌门(Spirochaetes)的相对丰度显著降低(P<0.05)。
图2 瘤胃门水平微生物相对丰度

Bacteroidetes:拟杆菌门;Firmicutes:厚壁菌门;Proteobacteria:变形菌门;Actinobacteria:放线菌门;Euryarchaeota:广古菌门;Verrucomicrobia:疣微菌门;Unspecified_Bacteria:未分类的细菌;Fibrobacteres:纤维杆菌门;Tenericutes:厚壁菌门;Lentisphaerae:黏胶球形菌门;Cyanobacteria:蓝菌门;Other:其他;Elusimicrobia:迷踪菌门;Synergistetes:互养菌门。

Fig.2 Rumen microbial relative abundance at phylum level

表6 瘤胃门水平微生物相对丰度(前15)

Table 6 Rumen microbial relative abundance at phylum level (top 15)%

项目
Items
组别 Groups SEM P
P-value
CON F1 F2 F3
拟杆菌门 Bacteroidetes 48.24c 67.76a 50.09c 64.79ab 0.11 0.03
厚壁菌门 Firmicutes 32.93 21.55 24.40 23.66 0.05 0.05
TM7 4.90 0.49 1.71 0.65 0.02 0.09
变形菌门 Proteobacteria 4.85 6.13 7.54 5.19 0.02 0.25
放线菌门 Actinobacteria 2.28a 0.41b 1.24ab 0.65b 0.01 0.04
互养菌门 Synergistetes 1.70 0.04 7.66 0.03 0.05 0.49
广古菌门 Euryarchaeota 1.21a 0.00c 1.17b 0.02c 0.24 0.02
厚壁菌门 Tenericutes 1.01 0.57 0.80 0.93 0.24 0.12
纤维杆菌门Fibrobacteres 0.67 0.59 1.19 0.88 0.63 0.78
疣微菌门Verrucomicrobia 0.50c 1.14b 1.49a 1.01b 0.67 0.04
蓝菌门 Cyanobacteria 0.43 0.49 0.63 0.88 0.31 0.53
未分类的细菌Unspecified_Bacteria 0.35 0.33 0.85 0.50 0.27 0.11
螺旋菌门 Spirochaetes 0.32a 0.08b 0.35a 0.08b 0.08 0.02
SR1 0.31 0.09 0.13 0.21 0.12 0.13
迷踪菌门 Elusimicrobia 0.16 0.18 0.08 0.31 0.21 0.20
表7可知,与CON组相比,F1、F3组的瘤胃中未明确分类的BS11属(unspecified_BS11)、未明确分类的RF16属(unspecified_RF16)和未明确分类的S24_7属(unspecified_S24_7)的相对丰度显著升高(P<0.05),未明确分类的毛螺菌科(unspecified_Lachnospiraceae)和未明确分类的韦荣式球菌科(unspecified_Veillonellaceae)的相对丰度显著降低(P<0.05);F2组的瘤胃中TG5的相对丰度显著升高(P<0.05)。
表7 瘤胃属水平微生物丰度(前15)

Table 7 Rumen microbial relative abundance at genus levels (top 15)%

项目
Items
组别 Groups SEM P
P-value
CON F1 F2 F3
普雷沃菌属 Prevotella 23.12 14.46 23.41 18.26 3.42 0.25
未明确分类的拟杆菌目
Unspecified_Bacteroidales
17.48 11.79 18.39 13.86 5.13 0.93
未明确分类的BS11属Unspecified_BS11 5.97b 17.36a 5.87b 16.98a 4.53 0.04
未明确分类的梭菌目
Unspecified_Clostridiales
5.00 3.21 3.38 3.06 1.11 0.33
未明确分类的瘤胃球菌科
Unspecified_Ruminococcaceae
5.00 4.31 6.13 3.98 1.08 0.27
未明确分类的F16属Unspecified_F16 4.90 0.49 1.71 0.65 1.83 0.13
未明确分类的毛螺菌科
Unspecified_Lachnospiraceae
3.29a 0.99b 2.12ab 0.63b 0.78 0.03
瘤胃球菌属Ruminococcus 2.76 1.76 1.75 1.55 0.49 0.14
颤螺菌属 Oscillospira 2.15 2.99 1.92 2.63 0.71 0.48
未明确分类的RF16属Unspecified_RF16 2.09b 6.51a 3.07ab 5.04a 1.63 0.04
CF231 2.02 2.29 1.65 2.24 0.75 0.82
未明确分类的韦荣式球菌科
Unspecified_Veillonellaceae
1.86a 0.33b 1.11ab 0.43b 0.57 0.03
TG5 1.70b 0.03b 7.64a 0.02b 4.76 <0.01
未明确分类的S24_7属
Unspecified_S24_7
1.57b 6.56a 2.10b 5.10a 0.75 <0.01
梭状芽孢杆菌属Clostridium 1.44ab 1.29ab 1.05b 1.67a 0.18 0.04

2.5 瘤胃微生物功能预测

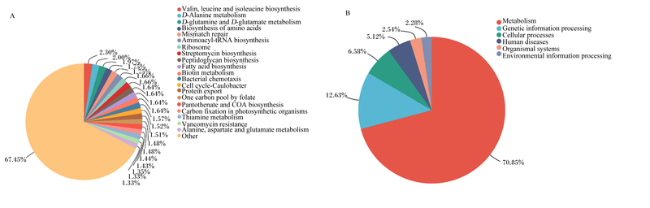
图3可知,瘤胃微生物功能基因相对丰度由高到低分别是缬氨酸、亮氨酸和异亮氨酸的生物合成,D-丙氨酸的代谢、D-谷氨酰胺和D-谷氨酸代谢,链霉素的生物合成和脂肪酸的生物合成等。将瘤胃微生物的功能基因进行分类,主要为新陈代谢功能。
图3 瘤胃微生物功能分析

Valin, leucine and isoleucine biosynthesis:缬氨酸、亮氨酸和异亮氨酸的生物合成;D-Alanine metabolism:D-丙氨酸的代谢;D-glutamine and D-glutamate metabolism:D-谷氨酰胺和D-谷氨酸代谢;Biosynthesis of amino acids:氨基酸的生物合成;Mismatch repair:异源双链修复;Aminoacyl-tRNA biosynthesis:氨基酸-tRNA生物合成;Ribosome:核糖体;Streptomycin biosynthesis:链霉素的生物合成;Peptidoglycan biosynthesis:肽聚生物合成;Fatty acid biosynthesis:脂肪酸的生物合成;Biotin metabolism:生物素的代谢;Bacterial chemotaxis:细菌耐药性;Cell cycle-Caulobacter:细胞周期-茎秆菌;Protein export:蛋白质输出;One carbon pool by folate:一个叶酸碳库;Pantothenate and COA biosynthesis:泛酸和辅酶A生物合成;Carbon fixation in photosynthetic organisms:光合生物的碳固定;Thiamine metabolism:硫胺素的代谢;Vancomycin resistance:万古霉素耐药性;Alanine, aspartate and glutamate metabolism:丙氨酸、天冬氨酸和谷氨酸的代谢;Metabolism:新陈代谢;Genetic information processing:遗传信息处理;Cellular processes:细胞过程;Human diseases:人类疾病;Organismal systems:有机系统;Environmental information processing:环境信息处理;Other:其他。

Fig.3 Analysis of microbial function in rumen

2.6 岩藻多糖对断奶羔羊瘤胃代谢物的影响

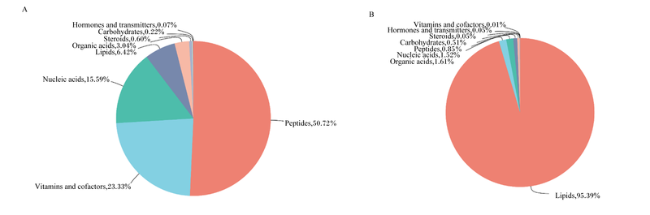
图4可知,在正、负离子模式下分析瘤胃代谢物的组成,正离子模式下的代谢物分为8类,由高到低依此为肽类、维生素和辅助因子类、核酸类、脂类、有机酸类、固醇类、碳水化合物类及激素和递质类;负离子模式下的代谢物也分为8类,由高到低依此为脂类、有机酸类、核酸类、肽类、碳水化合物类、固醇类、激素和递质类及维生素和辅助因子类。
图4 正、负离子模式下瘤胃代谢物组成分析

A:正离子模式 positive ion mode;B:负离子模式 negative ion mode。Hormones and transmitters:激素和递质类;Carbohydrates:碳水化合物类;Steroids:固醇类;Organic acids:有机酸类;Lipids:脂类;Nucleic acids:核酸类;Vitamins and cofactors:维生素和辅助因子类;Peptides:肽类。

Fig.4 Analysis of rumen metabolites composition in positive and negative ion mode

通过统计分析与正交偏最小二乘法判别分析(orthogonal partial least squares-discriminant analysis,OPLS-DA)来判定组间代谢物的差异,选取变量投影重要性(variable importance in projection,VIP)>1、P<0.05作为组间有显著差异的代谢物。由表8可知,正离子模式下组间差异排名前15的代谢物中,与CON组相比,F1、F2、F3组的瘤胃中碳水化合物类、肽类、核酸类及激素和递质类代谢物含量显著降低(P<0.05),有机酸类、维生素和辅助因子类、固醇类及脂类代谢物含量显著升高(P<0.05)。由表9可知,负离子模式下组间差异排名前15的代谢物中,与CON组相比,F1、F2、F3组的瘤胃中固醇类及激素和核酸类代谢物含量显著降低(P<0.05),其他类代谢物含量显著升高(P<0.05)。
表8 正离子模式下组间差异代谢物对比分析(前15)

Table 8 Comparative analysis of differential metabolites between groups in positive ion mode (top 15)%

项目
Items
组别 Groups 变量投影
重要性
VIP
P
P-value
CON F1 F2 F3
碳水化合物类 Carbohydrates
麦芽四糖 Maltotetraose 0.62a 0.29b 0.13c 0.07c 2.31 <0.01
D-葡萄糖 D-glucose 4.95a 1.83b 1.08c 0.73c 2.10 0.02
核酸类 Nucleic acids
葡萄糖-1-磷酸 Glucose 1-phosphate 4.40a 2.69b 1.47c 1.15d 2.00 0.04
D-氨基葡萄糖6-磷酸
D-glucosamine 6-phosphate
1.62a 0.93b 0.54c 0.41c 2.27 <0.01
维生素和辅助因子类 Vitamins and cofactors
组氨酸蛋白激酶 HPK 1.17c 1.27b 1.98a 1.96a 2.21 <0.01
水黄皮 Karanjin 5.57c 6.02b 8.17a 7.61ab 1.97 <0.01
高良姜素 Galangin 0.17c 0.20b 0.28a 0.26a 1.96 <0.01
4-吗啉-3-硝基苯-1-磺胺
4-morpholino-3-nitrobenzene-
1-sulfonamide
0.19c 0.25b 0.35a 0.32a 2.01 <0.01
3-(4-硝基苯基)[1,2,3]三唑
[1,5-α]喹唑林-5-胺
3-4(-nitrophenyl) [1,2,3]triazolo
[1,5-α]aquinazolin-5-amine
0.17c 0.19b 0.25a 0.29a 2.19 <0.01
固醇类 Steroids
甲睾酮 Methyltestosterone 0.33c 0.49b 0.69b 1.26a 2.14 0.03
激素和递质类 Hormones and transmitters
前列腺素G2 Prostaglandin G2 8.49a 6.82c 6.79c 7.71b 1.99 <0.01
肽类 Peptides
4-氨基-2-(甲基磺胺基)-1,3-
噻唑-5-羧酸乙酯
4-amino-2-(methylsulfanyl)-1,3-
thiazole-5-ethyl carboxylate
29.54a 21.91b 8.11c 4.63d 2.10 0.02
戊烷-3-甲基-5-[(2-氨基苯甲酰)
氨基]-2-氯-苯酸酯
Pentane-3-methyl-5-[(2-aminobenzoyl)
amino]-2-chlorobenzoate
5.00a 2.75c 4.60b 4.34b 2.05 <0.01
有机酸类 Organic acids
N-乙酰-L-缬氨酸 N-acetyl-L-valine 0.78c 0.87b 0.95a 1.07a 2.14 0.02
2-苄基丁二酸 2-benzyl succinic acid 0.19c 0.22b 0.29a 0.32a 1.99 0.04
表9 负离子模式下组间差异代谢物对比分析(前15)

Table 9 Comparative analysis of differential metabolites between groups in negative ion mode (top 15)%

项目
Items
组别 Groups 变量投影
重要性
VIP
P
P-value
CON F1 F2 F3
有机酸类 Organic acids
硬脂酸 Stearic acid 23.12d 35.01c 39.17b 44.98a 2.24 <0.01
甘草亭酸 Glycyrrhetinic acid 0.41c 0.45c 0.63ab 0.77a 2.23 <0.01
十五烷酸 Pentadecanoic acid 1 096.14c 1 049.39c 1 300.26b 1 678.66a 2.08 <0.01
十四烷二酸 Tetradecanedioic acid 1.99d 5.54c 15.04a 9.27b 1.93 <0.01
维生素和辅助因子类 Vitamins and cofactors
4H-1,2,4-三氮唑4H-1,2,4-triazol 0.92c 1.26b 1.45b 2.69a 2.23 0.02
4-吡哆酸 4-pyridoxic acid 0.36c 2.37b 3.62a 3.23ab 1.56 0.02
(±)苏式-9,10-二羟基-12(Z)-
十八碳烯酸
(±)-threo-9,10-dihydroxy-12(Z)-
octadecenoic acid
1.48c 3.13b 3.77a 3.06b 1.31 <0.01
固醇类 Steroids
肌醇 Inositol 9.60a 4.66b 1.57c 0.87d 2.16 0.03
激素和递质类 Hormones and transmitters
肾上腺酸 Adrenic acid 1.70d 1.92c 2.07b 2.98a 1.99 0.04
前列腺素D1 Prostaglandin D1 0.19c 0.22b 0.33a 0.25b 1.61 <0.01
前列腺素D2 Prostaglandin D2 36.39c 42.82b 59.09a 61.94a 1.14 0.03
13,14-二氢前列腺素E1
13,14-dihydro prostaglandin E1
9.48c 9.56b 16.40a 19.38a 2.16 <0.01
磷酸烯醇丙酮酸
Phosphoenol pyruvic acid
0.16c 0.94a 0.79b 0.92a 1.84 0.02
核酸类 Nucleic acids
6-羧基己酸 6-hydroxycaproic acid 2.46a 1.21c 1.57b 1.06c 1.61 0.03
肽类 Peptides
羟基脂肪酸支链脂肪酸酯
Hydroxyl fatty acid branched fatty acid ester
0.51d 0.62c 1.21b 1.65a 1.12 0.04

2.7 岩藻多糖对断奶羔羊瘤胃代谢通路分析

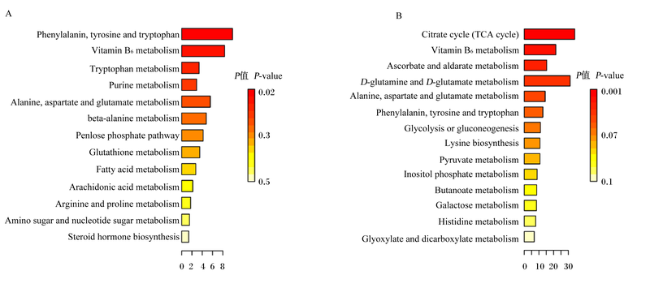
图5为正、负离子模式差异代谢物ORA通路富集图。由表10可知,正离子模式下苯丙氨酸、酪氨酸和色氨酸的生物合成和维生素B6代谢为差异代谢物参与的有显著差异的代谢通路(P<0.05),负离子模式下柠檬酸循环(三羧酸循环)、维生素B6代谢、抗坏血酸和醛酸代谢及D-谷氨酰胺和D-谷氨酸的代谢为差异代谢物参与的有显著差异的代谢通路(P<0.05)。
图5 正、负离子模式下差异代谢物ORA通路富集

A:正离子模式;B:负离子模式。横坐标是富集倍数,表示代谢通路中观测代谢数量/理论代谢物数量。用不同颜色表示P值大小,颜色越深P值越小。

Phenylalanin, tyrosine and tryptophan:苯丙氨酸、酪氨酸和色氨酸;Vitamin B6 metabolism:维生素B6代谢;Tryptophan metabolism:色氨酸代谢;Purine metabolism:嘌呤代谢;Alanine, aspartate and glutamate metabolism:丙氨酸、天冬氨酸和谷氨酸新陈代谢;beta-alanine metabolism:β-丙氨酸代谢;Penlose phosphate pathway:磷酸戊糖途径;Glutathione metabolism:谷胱甘肽代谢;Fatty acid metabolism:花生四烯酸代谢;Arginine and proline metabolism:精氨酸和脯氨酸代谢;Amino sugar and nucleotide sugar metabolism:氨基酸和核苷酸代谢;Steroid hormone biosynthesis:类固醇激素生物合成;Citrate cycle (TCA cycle):柠檬酸循环(三羧酸循环);Ascorbate and aldarate metabolism:抗坏血酸和藻酸盐代谢;D-glutamine and D-glutamate metabolism:D-谷氨酰胺和D-谷氨酸代谢;Glycolysis or gluconeogenesis:糖酵解;Lysine biosynthesis:赖氨酸生物合成;Pyruvate metabolism:丙酮酸代谢;Inositol phosphate metabolism:磷酸肌醇代谢;Butanoate metabolism:丁酸酯代谢;Galactose metabolism:半乳酸代谢;Histidine metabolism:组氨酸代谢;Glyoxylate and dicarboxylate metabolism:乙醛酸和二羧酸代谢。

Fig.5 Positive and negative ion mode difference metabolite ORA pathway enrichment

A: positive ion mode;B: negative ion mode. The abscissa is the fold enrich, which indicates the observed metabolic quantity/theoretical metabolite quantity in the metabolic pathway. Use different colors to represent the size of P-value, the darker the color, the smaller the P-value.

表10 代谢物显著差异代谢通路

Table 10 Metabolite significantly different pathways

项目
Items
富集倍数
Fold enrich
P
P-value
正离子模式 Positive ion mode
苯丙氨酸、酪氨酸和色氨酸的生物合成 Phenylalanine, tyrosine and tryptophan biosynthesis 9.91 0.02
维生素B6代谢 Vitamin B6 metabolism 8.36 0.02
负离子模式 Negative ion mode
柠檬酸循环(三羧酸循环) Citrate cycle (TCA cycle) 34.39 <0.01
维生素B6代谢 Vitamin B6 metabolism 21.49 <0.01
抗坏血酸和醛酸代谢 Ascorbate and aldarate metabolism 15.28 0.01
D-谷氨酰胺和D-谷氨酸的代谢 D-glutamine and D-glutamate metabolism 31.26 0.03

3 讨论

3.1 岩藻多糖对断奶后羔羊生长性能的影响

生长性能参数可以直观反映畜禽的经济价值,ADFI、ADG和F/G是反映生长性能的重要指标,是养分摄入、消化与吸收的最终表现[8]。Rattigan等[9]研究发现,断奶仔猪在食用添加了岩藻多糖的饲粮14 d后生长性能并未受到显著影响。研究发现,在断奶仔猪饲粮中添加500 mg/kg的岩藻多糖,仔猪的F/G显著降低[10]。王彦东[11]研究发现,断奶会降低羔羊生长性能和免疫力。本试验中,与CON组相比,F2、F3组的ADG和ADFI显著升高,F/G显著降低。虽然岩藻多糖在反刍动物上的应用较少,但本研究结果表明在断奶羔羊饲粮中添加岩藻多糖仍有类似的结果,可能因为岩藻多糖能改善胃肠道菌群,提高机体免疫,进而提高断奶后羔羊的生长性能。

3.2 岩藻多糖对断奶后羔羊瘤胃pH与挥发性脂肪酸含量的影响

瘤胃pH和挥发性脂肪酸含量可以综合评价瘤胃微生物区系和瘤胃代谢物的状况,是反映瘤胃发酵情况的重要指标[12]。吴璞等[13]研究表明,山羊瘤胃pH介于5.5~7.5。本试验断奶羔羊瘤胃pH介于6.6~6.9,处于正常范围内,说明饲粮中添加岩藻多糖以后并未使瘤胃pH产生异常。挥发性脂肪酸是反刍动物重要的能源之一,是由瘤胃微生物消化饲粮产生的。本研究中,与CON组相比,饲粮中添加岩藻多糖的试验组瘤胃乙酸、丁酸、异丁酸含量和乙酸/丙酸显著升高,与前人研究相类似。有研究表明,黄芪多糖可以显著提高羔羊瘤胃丙酸含量[14],也有报道说添加益生菌显著提高了瘤胃乙酸、丁酸含量和乙酸/丙酸[15]。这些研究表明,添加岩藻多糖与其他植物性多糖一样可以提高瘤胃挥发性脂肪酸含量,改善反刍动物瘤胃发酵功能。

3.3 岩藻多糖对断奶后羔羊瘤胃微生物区系的影响

瘤胃微生物对饲粮中营养物质消化、瘤胃发酵参数和反刍动物机体功能的维持有重要作用。有研究发现,添加猴头菇多糖能改善山羊瘤胃菌群结构,维持瘤胃健康[16]。本研究采用16S RNA测序技术对断奶后瘤胃中微生物多样性和组成进行检测,结果表明,岩藻多糖并没有显著改变断奶后羔羊瘤胃微生物多样性,这表明饲粮中添加岩藻多糖并不会造成断奶后羔羊瘤胃微生物紊乱。Jiang等[17]研究发现,添加功能性多糖能改善反刍动物瘤胃微生物菌群的多样性与相对丰度。这与本研究结果不同,可能是多糖的添加量、种类以及试验羊的品种与年龄不同导致的。本研究结果显示,各组羔羊间微生物组成有差异,各组间样本区分明显;在门水平上,断奶后羔羊瘤胃中Fimicutes和Bacteroidetes占瘤胃微生物总相对丰度的70%以上,为断奶后羔羊瘤胃微生物中的优势菌门,这与前人的研究结果[18-21]一致。饲粮中添加岩藻多糖提高了断奶后羔羊瘤胃中Bacteroidetes、Verrucomicrobia和Fibrobacteres的相对丰度,同时降低了Euryarchaeota的相对丰度。而Euryarchaeota是瘤胃中常见的菌门,包含多种产甲烷菌等。与本研究结果类似,马秀花等[22]在饲粮中添加甘露寡糖发现提高了滩羊瘤胃中Bacteridetes和Firmicutes的相对丰度,同时降低了瘤胃中变形菌门(Proteobacteria)的相对丰度。本研究进一步在属水平上发现,普雷沃菌属(Prevotella)和未明确分类的拟杆菌目(unspecified_Bacteroidales)为断奶后羔羊的优势菌属,这与李冲[23]报道的结果一致。另外,本试验结果表明岩藻多糖显著影响了部分菌属的相对丰度,与CON组相比,F1、F3组的瘤胃中unspecified_BS11、unspecified_RF16和unspecified_S24_7的相对丰度显著升高,unspecified_Lachnospiraceae和unspecified_Veillonellaceae的相对丰度显著降低。总体来说,与其他植物多糖效果类似,岩藻多糖能够改善断奶后羔羊瘤胃微生物菌群的相对丰度。

3.4 岩藻多糖对断奶后羔羊瘤胃代谢组学的影响

瘤胃代谢物与微生物关联,代谢组学相比基因组学和蛋白质组学更能较好解释表型的变化。大量研究表明,饲喂方式及饲粮添加剂会改变瘤胃的代谢物,而代谢物的改变可能与瘤胃微生物的相对丰度变化有关[24]。在本研究中,我们通过代谢组学分析了岩藻多糖对断奶后羔羊瘤胃内容物代谢物的影响,结果显示,与CON相比,添加岩藻多糖的试验组代谢物区分明显,这表明岩藻多糖改变了瘤胃代谢物的组成。对差异代谢通路分析发现,岩藻多糖引起了苯丙氨酸、酪氨酸和色氨酸的生物合成,维生素B6代谢,柠檬酸循环(三羧酸循环),抗坏血酸和醛酸代谢,D-谷氨酰胺和D-谷氨酸代谢5个相关代谢通路的改变。这些代谢通路涉及羔羊机体碳水化合物、氨基酸和维生素等的物质代谢。氨基酸对微生物的生长和代谢至关重要,是肽类和蛋白质合成的关键成分,还能够调节多种代谢通路[25]。苯丙氨酸、酪氨酸和色氨酸均为芳香族必需氨基酸,苯丙氨酸通过端粒酶的作用生成酪氨酸,是酪氨酸在体内合成的重要来源之一。有研究表明,瘤胃中酪氨酸含量与育肥绵羊生长性能呈正相关[26]。色氨酸在机体新陈代谢中起重要作用,能够产生多种生理活性物质并参与到机体生理活动与调节,如5-羟色酸、烟酸、生物碱、辅酶和褪黑素等。研究表明,瘤胃微生物能够合成B族维生素,且瘤胃中B组维生素含量同样能表明瘤胃微生物活性[27]。谷氨酰胺是血液和组织中游离氨基酸中含量最丰富的一种氨基酸,能够为组织上皮细胞提供能源物质,具有维持紧密连接蛋白和黏膜完整性、促进免疫细胞增殖及防止细菌移位等功能。研究表明,谷氨酰胺为反刍动物瘤胃上皮细胞提供能量[28]。刘玉洁等[29]报道,谷氨酰胺能够维持高精料饲粮下奶山羊瘤胃上皮的结构和形态,提高紧密连接功能并降低瘤胃上皮炎症反应。另外,谷氨酰胺与谷氨酸是瘤胃微生物利用氮途径中的关键物质。反刍动物瘤胃微生物利用氨主要通过2条途径完成,一条为α-酮戊二酸与谷氨酰胺脱氢酶(GDH)作用下生成谷氨酰胺的GDH途径,另一条为谷氨酸与氨在谷氨酰胺合成酶(GS)作用下转变为谷氨酰胺,然后谷氨酰胺和α-酮戊二酸在谷氨酸合成酶(GOGAT)作用下转变为谷氨酸的GS-GOGAT途径。此外,有研究表明,谷氨酰胺参与三羧酸循环代谢产生能量,谷氨酰胺在谷氨酸酶作下转变为谷氨酸,谷氨酸在转氨酶或GDH催化下转变为三羧酸循环的中间产物α-酮戊二酸[30]。总的来说,这些富集的通路为进一步研究岩藻多糖的具体调节机制提供数据和理论依据。

4 结论

饲粮中添加岩藻多糖提高了断奶羔羊的生长性能,改善了断奶羔羊瘤胃发酵,提高了瘤胃乙酸、丙酸、异丁酸、丁酸含量和乙酸/丙酸,在属水平上提高了unspecified_BS11、unspecified_RF16和unspecified_S24_7的相对丰度;改变了苯丙氨酸、酪氨酸和色氨酸的生物合成,维生素B6代谢,柠檬酸循环(三羧酸循环),抗坏血酸和醛酸代谢,D-谷氨酰胺和D-谷氨酸代谢5个相关代谢通路。
[1]
杨泓涛, 邓位喜, 杨玉能, 等. 黄芪多糖对舍饲黔北麻羊断奶羔羊生长性能、生化指标及免疫功能的影响[J]. 饲料研究, 2021, 44(9):29-32.

YANG H T, DENG W X, YANG Y N, et al. Effects of Astragalus polysaccharide on growth performance,biochemical indexes and immune function of weaned lambs of Qian Bei Ma sheep[J]. Feed Research, 2021, 44(9):29-32. (in Chinese)

[2]
史晨迪, 赵晓雅, 田沛知, 等. 羔羊断奶应激期饲喂方式对其生长性能和血清生化指标的影响[J]. 动物营养学报, 2022, 34(6):3799-3813.

DOI

SHI C D, ZHAO X Y, TIAN P Z, et al. Effects of feeding methods on growth performance and serum biochemical indices of lambs during weaning stress period[J]. Chinese Journal of Animal Nutrition, 2022, 34(6):3799-3813. (in Chinese)

DOI

[3]
ASCHENBACH J R, PENNER G B, STUMPFF F, et al. Ruminant nutrition symposium:role of fermentation acid absorption in the regulation of ruminal pH[J]. Journal of Animal Science, 2011, 89(4):1092-1107.

DOI

[4]
YÁÑEZ-RUIZ D R, ABECIA L, NEWBOLD C J. Manipulating rumen microbiome and fermentation through interventions during early life:a review[J]. Frontiers in Microbiology, 2015, 6:1133.

[5]
JING X P, WANG W J, DEGEN A, et al. Tibetan sheep have a high capacity to absorb and to regulate metabolism of SCFA in the rumen epithelium to adapt to low energy intake[J]. British Journal of Nutrition, 2020, 123(7):721-736.

DOI

[6]
SUN Y Y, CHENG M, XU M, et al. The effects of subacute ruminal acidosis on rumen epithelium barrier function in dairy goats[J]. Small Ruminant Research, 2018, 169:1-7.

DOI

[7]
QUIJADA N M, BODAS R, LORENZO J M, et al. Dietary supplementation with sugar beet fructooligosaccharides and garlic residues promotes growth of beneficial bacteria and increases weight gain in neonatal lambs[J]. Biomolecules, 2020, 10(8):1179.

DOI

[8]
刘绘汇, 孙康, 范慧玉, 等. 代乳粉中添加单宁酸对湖羊羔羊生长性能、养分表观消化率和肌肉脂肪酸组成的影响[J]. 动物营养学报, 2021, 33(8):4520-4532.

DOI

LIU H H, SUN K, FAN H Y, et al. Effects of tannic acid addition in milk replacer on growth performance,nutrient apparent digestibility and muscle fatty acid composition of Hu lambs[J]. Chinese Journal of Animal Nutrition, 2021, 33(8):4520-4532. (in Chinese)

[9]
RATTIGAN R, SWEENEY T, VIGORS S, et al. The effect of increasing inclusion levels of a fucoidan-rich extract derived from Ascophyllum nodosum on growth performance and aspects of intestinal health of pigs post-weaning[J]. Marine Drugs, 2019, 17(12):680.

DOI

[10]
刘萍, 赵金标, 耿正颖, 等. 日粮添加褐藻糖胶对断奶仔猪抗炎能力和肠道微生物多样性的影响[J]. 微生物学报, 2019, 59(4):700-710.

LIU P, ZHAO J B, GENG Z Y, et al. Influence of dietary fucoidan on inflammatory response and intestinal microbial diversity in weaned pigs[J]. Acta Microbiologica Sinica, 2019, 59(4):700-710. (in Chinese)

[11]
王彦东. 丁酸钠释放速率对犊牛抗氧化功能、免疫机能和断奶应激的影响[D].硕士学位论文. 呼和浩特: 内蒙古农业大学, 2020.

WANG Y D. Effects of release rate of sodium butyrate on anti-oxidative function,immune function and weaning stress of calves[D].Master's Thesis. Hohhot: Inner Mongolia Agricultural University, 2020. (in Chinese)

[12]
庞凯悦, 戴东文, 杨英魁, 等. 不同饲养方式对牦牛瘤胃发酵参数及微生物菌群的影响[J]. 动物营养学报, 2022, 34(3):1667-1682.

DOI

PANG K Y, DAI D W, YANG Y K, et al. Effects of different feeding methods on rumen fermentation parameters and microbial flora of yaks[J]. Chinese Journal of Animal Nutrition, 2022, 34(3):1667-1682. (in Chinese)

[13]
吴璞, 曹旭亮, 王虎成, 等. 红豆草茬地放牧对湖羊和小尾寒羊生长性能、瘤胃内环境参数及微生物区系的影响[J]. 动物营养学报, 2022, 34(3):1730-1742.

DOI

WU P, CAO X L, WANG H C, et al. Effects of grazing on stubble sainfoin pasture on growth performance,rumen environmental parameters and microflora of Hu sheep and small-tailed Han sheep[J]. Chinese Journal of Animal Nutrition, 2022, 34(3):1730-1742. (in Chinese)

[14]
ZHONG R Z, YU M, LIU H W, et al. Effects of dietary Astragalus polysaccharide and Astragalus membranaceus root supplementation on growth performance,rumen fermentation,immune responses,and antioxidant status of lambs[J]. Animal Feed Science and Technology, 2012, 174(1/2):60-67.

DOI

[15]
张志军. 复合益生菌制剂对绵羊瘤胃发酵、血清生化和奶牛生产性能的影响[D].硕士学位论文. 乌鲁木齐: 新疆农业大学, 2012.

ZHANG Z J. Effect of dietary compound probiotics on rumen fermentation,serum biochemistry of sheep and productive performance of dairy cow[D].Master's Thesis. Urumqi: Xinjiang Agricultural University, 2012. (in Chinese)

[16]
李颖. 猴头菇多糖缓解山羊亚急性瘤胃酸中毒效果及作用机理[D].硕士学位论文. 福州: 福建农林大学, 2019.

LI Y. The effect and mechanism of Hericium erinaceus polysaccharides mitigating SARA in goat[D].Master's Thesis. Fuzhou: Fujian Agriculture and Forestry University, 2019. (in Chinese)

[17]
JIANG C X, DING L M, DONG Q M, et al. Effects of root extracts of three traditional Chinese herbs as dietary supplements on dry matter intake,average daily gain,rumen fermentation and ruminal microbiota in early weaned yak calves[J]. Animal Feed Science and Technology, 2021, 278:115002.

[18]
金鹿, 李胜利, 桑丹, 等. 沙蒿多糖组合制剂对滩羊羔羊瘤胃菌群多样性的影响[J]. 动物营养学报, 2021, 33(1):317-329.

DOI

JIN L, LI S L, SANG D, et al. Effects of Artemisia polysaccharide combination preparation on rumen microflora diversity of Tan lambs[J]. Chinese Journal of Animal Nutrition, 2021, 33(1):317-329. (in Chinese)

[19]
王文文, 王园, 孟子琪, 等. 发酵麸皮多糖对杜寒杂交肉羊瘤胃菌群及其屏障功能相关指标的影响[J]. 动物营养学报, 2022, 34(1):640-650.

DOI

WANG W W, WANG Y, MENG Z Q, et al. Effects of fermented wheat bran polysaccharides on microbiota and rumen barrier junction related indices of Dorper×thin-tailed Han crossbred meat lambs[J]. Chinese Journal of Animal Nutrition, 2022, 34(1):640-650. (in Chinese)

[20]
圣平, 计少石, 何力, 等. 饲喂杂交构树对于湖羊瘤胃微生物群落组成的影响[J]. 饲料研究, 2021, 44(6):6-10.

SHENG P, JI S S, HE L, et al. Effect of hybrid Broussonetia papyrifera on rumen microbial community composition in Hu sheep[J]. Feed Research, 2021, 44(6):6-10. (in Chinese)

[21]
CHEN H, GUO B B, YANG M R, et al. Response of growth performance,blood biochemistry indices,and rumen bacterial diversity in lambs to diets containing supplemental probiotics and Chinese medicine polysaccharides[J]. Frontiers in Veterinary Science, 2021, 8:681389.

[22]
马秀花, 桂瑞麒, 焦娜, 等. 荞麦秸秆饲粮条件下甘露寡糖对滩羊瘤胃菌群结构的影响[J]. 动物营养学报, 2021, 33(4):2365-2377.

DOI

MA X H, GUI R Q, JIAO N, et al. Effect of mannan oligosaccharides on rumen bacterial flora structure of Tan sheep under buckwheat straw diet condition[J]. Chinese Journal of Animal Nutrition, 2021, 33(4):2365-2377. (in Chinese)

[23]
李冲. 断奶应激对羔羊消化道结构与功能发育的影响及其机理研究[D].博士学位论文. 兰州: 兰州大学, 2019.

LI C. Effects of weaning stress on the structural and functional development of digestive tract of lamb and its mechanism[D]. Ph.D.Thesis. Lanzhou: Lanzhou University, 2019. (in Chinese)

[24]
张振威, 朱明霞, 王长法. 异位酸影响反刍动物瘤胃代谢和生产性能的研究进展[J]. 动物营养学报, 2022, 34(3):1408-1415.

DOI

ZHANG Z W, ZHU M X, WANG C F. Effects of isoacids on ruminal metabolism and performance in rumiants:a review[J]. Chinese Journal of Animal Nutrition, 2022, 34(3):1408-1415. (in Chinese)

[25]
ANDERSEN T O, KUNATH B J, HAGEN L H, et al. Rumen metaproteomics:closer to linking rumen microbial function to animal productivity traits[J]. Methods, 2021, 186:42-51.

DOI

[26]
DE PAIVA FERREIRA A V, COMINOTTE A, LADEIRA M M, et al. Feedlot diets with soybean oil,selenium and vitamin E alters rumen metabolism and fatty acids content in steers[J]. Animal Feed Science and Technology, 2020, 260:114362.

[27]
石志斌, 赵静, 朱贵冠. 日粮添加大豆油、硒和维生素E对肉牛瘤胃代谢和体内脂肪酸含量的影响[J]. 中国饲料, 2020(6):76-80.

SHI Z B, ZHAO J, ZHU G G. Effects of dietary supplementation with soybean oil,selenium and vitamin E on rumen metabolism and fatty acid content in beef cattle[J]. China Feed, 2020(6):76-80. (in Chinese)

[28]
HONAN M C, GREENWOOD S L. Characterization of variations within the rumen metaproteome of Holstein dairy cattle relative to morning feed offering[J]. Scientific Reports, 2020, 10(1):3179.

DOI PMID

[29]
刘玉洁, 刘军花, 许婷婷, 等. 谷氨酰胺对饲喂高精料的奶山羊瘤胃上皮的保护效应研究[J]. 草业学报, 2014, 23(4):293-299.

LIU Y J, LIU J H, XU T T, et al. The effect of glutamine supplementation on the barrier function of ruminal epithelium during high grain diet feeding in dairy goats[J]. Acta Prataculturae Sinica, 2014, 23(4):293-299. (in Chinese)

[30]
PENG M L, HAN J, LI L L, et al. Metabolomics reveals the mechanism of (-)-hydroxycitric acid promotion of protein synthesis and inhibition of fatty acid synthesis in broiler chickens[J]. Animal, 2018, 12(4):774-783.

DOI PMID

Outlines

/