REVIEW

Research Progress of N-Carbamoyl Glutamate in Alleviating Intestinal Oxidative Stress in Pigs

  • HU Naizhi ,
  • MA Wenfeng , * ,
  • MAO Pei ,
  • WU Qiujue
Expand
  • College of Animal Science and Technology, Henan University Science and Technology, Luoyang 471000, China
*associate professor, E-mail:

Received date: 2022-09-09

  Online published: 2023-04-12

Abstract

The intestine is the intersection between the internal and external environment of the body. It is influenced by various factors such as feed, drinking water and environmental conditions, which results in the accumulation of reactive oxygen species (ROS) radicals in the body, thus leads to the occurrence of intestinal oxidative stress. N-carbamyl glutamate (NCG) is a structural analogue of N-acetyl glutamate, which can activate the rate-limiting enzyme of arginine synthesis and promote the synthesis of endogenous arginine in the intestine. Recent studies have found that NCG plays an important role in alleviating intestinal oxidative stress and maintaining intestinal health in pigs. This paper reviews the mechanism of NCG in relieving oxidative stress in pig intestines, and also provides a reference for the application of NCG in relieving oxidative stress in swine production.[Chinese Journal of Animal Nutrition, 2023, 35(4):2081-2086]

Cite this article

HU Naizhi , MA Wenfeng , MAO Pei , WU Qiujue . Research Progress of N-Carbamoyl Glutamate in Alleviating Intestinal Oxidative Stress in Pigs[J]. Chinese Journal of Animal Nutrition, 2023 , 35(4) : 2081 -2086 . DOI: 10.12418/CJAN2023.195

氧化应激是机体氧化还原系统被破坏的一种生理状态,引起活性氧自由基在体内累积,进而氧化DNA、脂质、蛋白质等分子的不饱和结构,导致机体代谢紊乱[1]。肠道是机体与外界环境进行物质、信息交换的主要场所,易受环境中有害菌、病毒等因子刺激,使细胞线粒体内活性氧(reactive oxygen species,ROS)含量急剧增加,造成肠道氧化还原系统失衡,对动物生产性能、生理机能造成不利影响,严重时可导致坏死性肠炎、溃疡等多种肠道疾病发生,制约猪的正常生长[2]
N-氨甲酰谷氨酸(N-carbamyl glutamate,NCG)与N-乙酰谷氨酸(N-acetylglutamate,NAG)可激活线粒体中氨基甲酰磷酸合成酶-Ⅰ(carbamoyl phosphate synthetase-Ⅰ,CPS-Ⅰ)和吡咯啉-5-羧酸合成酶(pyrroline-5-carboxylate synthase,P5CS)[3],促进谷氨酰胺和脯氨酸合成瓜氨酸,而瓜氨酸是合成精氨酸的主要前体,进而促进精氨酸的内源合成[4]。近些年,以仔猪[5]、大鼠[6]、羔羊[7]为试验动物时,发现NCG在提高机体抗氧化能力、缓解肠道氧化应激方面发挥关键作用。因此,本文总结了NCG缓解肠道氧化应激的可能机理及在生猪生产中的一些应用进展。

1 NCG缓解肠道氧化应激的机制

在规模化养殖环境下,氧化应激是引起猪生产性能降低的主要因素之一[8]。核因子E2相关因子2(nuclear factor erythroid 2-related factor 2,Nrf2)和谷胱甘肽是细胞内氧化还原平衡的主要调节因子,同时也是介导肠道氧化应激反应的主要代谢途径[9-10]。Zhang等[7]在羔羊的研究发现,NCG可以提高肠道Nrf2和谷胱甘肽过氧化物酶(glutathione peroxidase,GSH-Px)的表达,同时其与精氨酸代谢关系密切。因此,一般认为NCG是通过介导肠道精氨酸的代谢反应,从而调节机体的氧化还原状态。

1.1 NCG促进精氨酸合成缓解肠道氧化应激

Ahmad等[11]研究发现,ROS和丙二醛(malondialdehyde,MDA)积累与精氨酸的摄入量呈显著负相关,表明精氨酸可以参与清除ROS的反应过程。而对于幼龄仔猪而言,线粒体内NAG浓度较低,造成精氨酸合成限速酶P5CS的表达受到抑制,相应地限制了肠道精氨酸的合成效率[12]。然而,NCG具备与NAG相似的代谢途径,可以在肠道内激活P5CS,从而促进精氨酸的稳定合成[13]。精氨酸属于碱性氨基酸,其孤电子对位于胍基基团,与ROS结合后,可以影响机体的氧化还原状态[14]
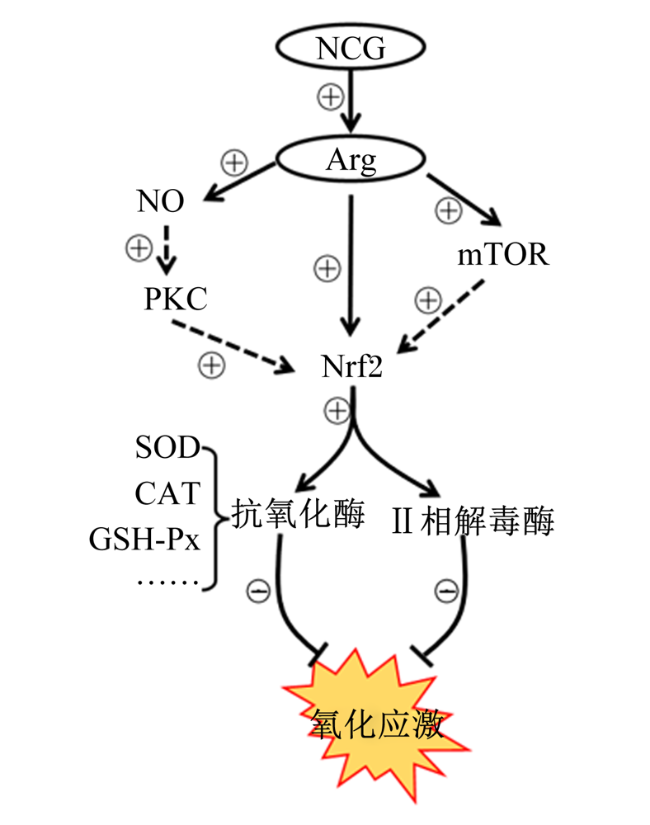
目前,Kelch样环氧氯丙烷相关蛋白1(Kelch like ECH associated protein 1,Keap1)/Nrf2信号通路被认为是缓解猪肠道细胞氧化损伤的重要途径,在正常生理状态下,Keap1可以快速分解Nrf2。Liang等[15]研究表明,精氨酸可抑制大鼠肠道Keap1和泛素连接酶3(CULLIN3)基因的表达,从而抑制Keap1识别和降解Nrf2,提高Nrf2入核数量;Nrf2也可通过提高谷氨酸半胱氨酸连接酶(glutamate cysteine ligase,GCL)和谷氨酸半胱氨酸连接酶(glutamate cysteine ligase,GCL)等谷胱甘肽合成酶基因的表达,相应地促进GSH的合成。此外,Mo等[16]研究发现,精氨酸能够上调大鼠脾脏的哺乳动物雷帕霉素靶蛋白(mechanistic target of rapamycin kinase,mTOR)基因表达,而mTOR是Nrf2的上游信号分子,可能正向调控Nrf2的表达。此外,Um等[17]研究表明,一氧化氮(NO)也可诱导细胞中Nrf2的表达,可能是通过激活蛋白激酶C(protein kinase C,PKC),进而促进Keap1的S-亚硝化,提高Nrf2的表达量。同时,NCG可促进育肥猪机体NO的生成[18],但是否能激活PKC介导Nrf2的表达还有待进一步研究。因此,一般认为NCG可以介导精氨酸的合成,进而影响Keap1/Nrf2信号通路关键蛋白的表达,从而相应地缓解肠道氧化反应(图1)。
图1 NCG介导Nrf2信号通路缓解肠道氧化应激

NCG:N-氨甲酰谷氨酸 N-carbamyl glutamate;Arg:精氨酸 arginine;mTOR:哺乳动物雷帕霉素靶蛋白 mammalian target of rapamycin;Nrf2:核因子E2相关因子2 nuclear factor erythroid 2-related factor 2;SOD:超氧化物歧化酶 superoxide dismutase;CAT:过氧化氢酶 catalase;GSH-Px:谷胱甘肽过氧化酶 glutathione peroxidase。

Fig.1 NCG-mediated Nrf2 signaling pathway relieves intestinal oxidative stress[13,15-18]

1.2 NCG介导谷胱甘肽合成途径缓解肠道氧化应激

谷胱甘肽是谷氨酸、半胱氨酸和甘氨酸组成的三肽,同时也是动物细胞中含量丰富的一类小分子硫醇,在清除自由基、阻止脂质过氧化、降低线粒体DNA损伤等方面发挥作用[19]。谷胱甘肽抗氧化系统是由谷胱甘肽还原型(GSH)和氧化型(GSSG)组成,通过2种形式之间的相互转换调节细胞氧化还原平衡[20]。GSH在GSH-Px或谷胱甘肽转移酶(glutathione S-transferase,GST)的作用下,与ROS和脂质过氧化物发生反应后,被氧化为GSSG;而GSSG在谷胱甘肽还原酶(glutathione reductase,GR)的作用下被还原成GSH[21]。肠道受到大量ROS胁迫时,GSH与GSSG的动态平衡被打破,引起机体的氧化反应,研究表明,NCG可调控谷胱甘肽抗氧化系统,参与清除肠道中的ROS,保护肠上皮细胞免于氧化损伤[16]
Mo等[16]研究发现,氧化应激大鼠饲喂NCG后,能够提高肠道GR的活性,相应地促进GSSG还原为GSH。Zhang等[7]也在报道中指出,NCG可提高空肠GSH-Px的活性,增强机体清除ROS和MDA的能力。另外,GCL和GS是GSH合成的关键限速酶,GSH合成酶的激活被认为在调控氧化应激中发挥关键作用[10]。Zhang等[22]研究发现,羔羊哺乳期添加NCG,GSH和GSH/GSSG比值在十二指肠、空肠、回肠中的数值显著提高,同时小肠MDA含量显著降低,相应地介导机体的氧化状态。然而,关于NCG在调控猪肠道谷胱甘肽合成的研究相对较少。

1.3 NCG介导NO代谢途径缓解肠道氧化应激

NO是机体分布最广泛的信号分子,在许多生理和病理过程中发挥着关键的调控作用[23]。有研究表明,NO在机体代谢中可以清除ROS,在肠道内,NO与超氧阴离子( O 2 -)反应后,生成了过氧亚硝酸盐(ONOO-),之后转化为 NO 2 - N O 3 -,从而排出体外。另外,NO也是重要的血管扩张剂。在乙酰胆碱作用下,NO由血管内皮细胞释放出来,相应地降低了血管张力,缓解了氧化应激引起的肠道缺氧问题[24]。此外,NO代谢途径还可激活抗氧化相关因子,调控机体和细胞的氧化应激反应[25]。在机体中,精氨酸、 还原型烟酰胺腺嘌呤二核苷酸磷酸(nicotinamide adenine dinucleotide phosphate,NADPH)和氧气在一氧化氮合酶(nitric oxide synthase,NOS)的催化下合成NO,而NOS是NO的唯一限速酶;在肠道精氨酸缺乏的情况下,NOS可以催化氧气生成 O 2 -,增加ROS的产生[26]。Cai等[27]研究发现,NCG可通过精氨酸-NO途径提高猪肠道内皮型一氧化氮合酶(endothelia nitric oxide synthase,eNOS)的表达水平,促进机体NO生成。

2 NCG在缓解生猪氧化应激上的应用

2.1 NCG用于缓解母猪氧化应激

由于猪缺乏功能性汗腺、体重较大且皮下脂肪较厚,阻碍了自身向外分散热量,造成体内积热,诱发热应激。在母猪妊娠后期和哺乳期,由于机体代谢旺盛而更易出现热应激[28]。热应激导致母猪采食量下降、代谢耗能增加,从而导致能量负平衡,使得线粒体功能负荷增加,进而导致氧化应激[29]。氧化应激损伤了母猪机体健康,从而直接或间接地对卵子及胚胎发育产生不良影响,抑制了母猪繁殖性能的发挥[30]。也有研究发现,NCG可以缓解由于氧化应激引起的母猪繁殖性能下降[31-33]
Zhu等[31]研究发现,初产母猪妊娠前期补充NCG,增加了子宫血流量,显著提高妊娠28 d胚胎着床数和胚胎存活数,显著降低胚胎死亡率,提高胚胎着床和发育相关的蛋白表达,也上调了eNOS、过氧化还蛋白6(peroxiredoxin 6,PRDX6)、热休克蛋白70(heat shock protein 70,Hsp70)等与抗氧化相关蛋白的表达,表明NCG可以缓解母猪的氧化应激反应。Feng等[32]报道指出,在母猪妊娠后期和哺乳期添加0.05% NCG,可提高仔猪初生窝重和平均活仔重,以及降低母体循环中的MDA和皮质醇含量。Liu等[33]在母猪宫内生长受限(IUGR)的研究中发现,在妊娠期母猪饲粮中添加0.1% NCG,可提高脐静脉血管内皮生长因子A(vascular endothelial growth factor A,VEGF-A)和eNOS基因的表达,提高脐静脉运输氧气和营养物质的能力,缓解母猪氧化应激引起的宫内生长受限。

2.2 NCG用于缓解仔猪氧化应激

仔猪在出生和断奶阶段由于环境突然变化易导致氧化应激。在出生阶段,由从子宫内低氧迅速转变到子宫外高氧的环境中,造成胎儿呼吸系统的线粒体产生大量ROS,然而,新生仔猪体内NAG活性较低,体内抗氧化系统无法完全清除ROS[34]。而在14日龄左右,仔猪机体的NAG活性恢复至正常水平;28日龄断奶阶段,仔猪面临了营养、心理、环境等多种应激叠加,机体抗氧化酶活性显著下降,肠道发生了较高的氧化应激反应,而内源精氨酸的合成量仍不足以清除断奶阶段产生的大量ROS[35-36]。研究发现,氧化应激会破坏仔猪肠道形态和免疫功能,对肠道的损伤作用可以一直延续至成年猪阶段[35,37],而NCG可直接促进仔猪内源精氨酸的合成,有利于缓解仔猪生理阶段的氧化应激[5]
Cai等[27]报道指出,在妊娠早期母猪饲粮中添加0.05% NCG,可改善羊水和血清中谷胱甘肽代谢,缓解ROS对胚胎的胁迫,最终保护胚胎免受氧化应激。Zhang等[38]探究了在大肠杆菌应激条件下,NCG对新生仔猪肠道黏膜免疫功能的影响,发现灌服50 mg/kg BW NCG提高了血浆精氨酸和黏膜分泌型免疫球蛋白(SIgA)含量,降低了肠道MDA和过氧化氢含量,从而提高了肠道抗氧化能力和免疫功能。由于NCG在新生仔猪上的应用较少,而补充NCG或精氨酸均可以提高血浆精氨酸含量,且NCG的半衰期较长,相较于精氨酸,能持续稳定增加内源精氨酸的合成[39-40]。此外,在饲粮中使用NCG,还可以避免精氨酸与其他碱性氨基酸吸收时的拮抗作用。
Wu等[39]研究表明,在断奶仔猪饲粮中添加0.08% NCG后,肠道HSP70在mRNA和蛋白质水平上的表达都得到了增强,相应地减少肠道应激反应,从而提高仔猪的生长性能。Yang等[40]研究发现,在21日龄断奶的环江小型猪为研究对象时,饲粮中添加0.1% NCG,血浆精氨酸含量显著提高,空肠溶质载体家族6成员19(solute carrier family 6 member 19,Slc6a19)、溶质载体家族7成员9(solute carrier family 7 member 9,Slc7a9)和溶质载体家族1成员1(solute carrier family 7 member 9,Slc1a1)的mRNA丰度显著提高,相应地影响断奶仔猪肠道的消化吸收能力。

2.3 NCG用于缓解生长育肥猪氧化应激

在生长育肥猪阶段,猪舍饲养密度和卫生、冷热应激、运输应激和真菌毒素等均会引起氧化应激反应,严重时引起生长育肥猪生长性能下降、肉品质受损和货架期缩短等问题[8]。目前,围绕NCG缓解生长育肥猪氧化应激的研究报道较少,主要集中在调控生长育肥猪的肉品质方面。
Yi等[41]研究表明,在生长育肥猪饲粮中添加1%精氨酸可缓解热应激导致的肠道损伤,提高空肠上皮细胞黏蛋白-2、闭锁小带蛋白-1(ZO-1)、阻滞素蛋白的表达,改善了生长育肥猪小肠的屏障功能。Ye等[42]报道指出,低蛋白质饲粮添加NCG后,显著提高了肥育猪的无脂瘦肉增重,同时增加了背最长肌的亮氨酸含量。Xing等[43]研究发现,NCG可以减少宁乡猪皮下脂肪沉积,提高背最长肌油酸、α-亚麻酸和泡桐酸的含量,降低花生四烯酸含量,提升宁乡猪肉品质。

3 小结与展望

综上所述,NCG在维持猪肠道精氨酸稳态、调控肠道氧化平衡状态等方面发挥重要作用,可以缓解由于氧化应激带来的不同阶段猪生产性能下降等问题。由于精氨酸在胃中降解率高,需要包被,导致其使用成本较高。NCG相较于精氨酸在胃液降解率低,添加量小,生产成本低,且不易与赖氨酸、组氨酸等碱性氨基酸产生拮抗作用。然而,NCG在缓解单胃动物氧化应激、调控肠道细胞增殖的研究较少,此外,大多数研究局限于NCG对精氨酸的调控作用,对于NCG调控精氨酸合成以外的机制几乎没有涉及。随着生物技术手段的不断发展,进一步探索NCG调控单胃动物肠道氧化应激的分子作用机制,有助其更好地应用于畜禽生产。
[1]
OTT M, GOGVADZE V, ORRENIUS S, et al. Mitochondria,oxidative stress and cell death[J]. Apoptosis, 2007, 12(5):913-922.

DOI

[2]
CIRCU M L, AW T Y. Intestinal redox biology and oxidative stress[J]. Seminars in Cell & Developmental Biology, 2012, 23(7):729-737.

[3]
DANIOTTI M, LA MARCA G, FIORINI P, et al. New developments in the treatment of hyperammonemia:emerging use of carglumic acid[J]. International Journal of General Medicine, 2011, 4:21-28.

[4]
CHACHER B, LIU H Y, WANG D M, et al. Potential role of N-carbamoyl glutamate in biosynthesis of arginine and its significance in production of ruminant animals[J]. Journal of Animal Science and Biotechnology, 2013, 4(1):16.

DOI PMID

[5]
高运苓. N-氨甲酰谷氨酸缓解仔猪早期断奶应激及促生长作用机理研究[D]. 硕士学位论文. 北京: 中国科学院大学, 2010.

GAO Y L. Study on mechanism of N-carbamoyl glutamate alleviating early weaning stress and promoting growth of piglets[D]. Master's Thesis. Beijing: University of Chinese Academy of Sciences, 2010. (in Chinese)

[6]
XIAO L, CAO W, LIU G M, et al.Arginine, N-carbamylglutamate, and glutamine exert protective effects against oxidative stress in rat intestine[J]. Animal Nutrition, 2016, 2(3):242-248.

DOI

[7]
ZHANG H, SUN H, PENG A, et al. N-carbamylglutamate and L-arginine promote intestinal function in suckling lambs with intrauterine growth restriction by regulating antioxidant capacity via a nitric oxide-dependent pathway[J]. Food & Function, 2019, 10(10):6374-6384.

[8]
HAO Y, XING M J, GU X H. Research progress on oxidative stress and its nutritional regulation strategies in pigs[J]. Animals, 2021, 11(5):1384.

DOI

[9]
WEN Z Y, LIU W H, LI X, et al. A protective role of the NRF2-Keap1 pathway in maintaining intestinal barrier function[J]. Oxidative Medicine and Cellular Longevity, 2019, 2019:1759149.

[10]
DIAZ-VIVANCOS P, DE SIMONE A, KIDDLE G, et al. Glutathione—linking cell proliferation to oxidative stress[J]. Free Radical Biology and Medicine, 2015, 89:1154-1164.

DOI

[11]
AHMAD A, SATTAR M Z A, RATHORE H A, et al. Antioxidant activity and free radical scavenging capacity of L-arginine and NaHS:a comparative in vitro study[J]. Acta Poloniae Pharmaceutica, 2015, 72(2):245-252.

[12]
GENG M M, LI T J, KONG X F, et al. Reduced expression of intestinal N-acetylglutamate synthase in suckling piglets:a novel molecular mechanism for arginine as a nutritionally essential amino acid for neonates[J]. Amino Acids, 2011, 40(5):1513-1522.

DOI

[13]
CHACHER B, ZHU W, YE J A, et al. Effect of dietary N-carbamoylglutamate on milk production and nitrogen utilization in high-yielding dairy cows[J]. Journal of Dairy Science, 2014, 97(4):2338-2345.

DOI PMID

[14]
XU N J, CHEN G Q, LIU H. Antioxidative categorization of twenty amino acids based on experimental evaluation[J]. Molecules, 2017, 22(12):2066.

DOI

[15]
LIANG M C, WANG Z X, LI H, et al. L-arginine induces antioxidant response to prevent oxidative stress via stimulation of glutathione synthesis and activation of Nrf2 pathway[J]. Food and Chemical Toxicology, 2018, 115:315-328.

DOI PMID

[16]
MO W W, WU X J, JIA G, et al. Roles of dietary supplementation with arginine or N-carbamylglutamate in modulating the inflammation,antioxidant property,and mRNA expression of antioxidant-relative signaling molecules in the spleen of rats under oxidative stress[J]. Animal Nutrition, 2018, 4(3):322-328.

DOI

[17]
UM H C, JANG J H, KIM D H, et al. Nitric oxide activates Nrf2 through S-nitrosylation of Keap1 in PC12 cells[J]. Nitric Oxide, 2011, 25(2):161-168.

DOI

[18]
WANG C P, SHANG L J, GUO Q P, et al. Effectiveness and safety evaluation of graded levels of N-carbamylglutamate in growing-finishing pigs[J]. Animal Nutrition, 2022, 10:412-418.

DOI PMID

[19]
MEISTER A. Biosynthesis and functions of glutathione,an essential biofactor[J]. Journal of Nutritional Science and Vitaminology, 1992, 38(Special):1-6.

[20]
KAPLOWITZ N, AW T Y, OOKHTENS M. The regulation of hepatic glutathione[J]. Annual Review of Pharmacology and Toxicology, 1985, 25:715-744.

PMID

[21]
LU S C. Glutathione synthesis[J]. Biochimica et Biophysica Acta-General Subjects, 2013, 1830(5):3143-3153.

DOI

[22]
ZHANG H, ZHAO F F, PENG A L, et al. Effects of dietary L-arginine and N-carbamylglutamate supplementation on intestinal integrity,immune function,and oxidative status in intrauterine-growth-retarded suckling lambs[J]. Journal of Agricultural and Food Chemistry, 2018, 66(16):4145-4154.

DOI

[23]
HANCOCK J T, VEAL D. Nitric oxide,other reactive signallingcompounds,redox,and reductive stress[J]. Journal of Experimental Botany, 2021, 72(3):819-829.

DOI

[24]
RAGHAVAN S A V, DIKSHIT M. Vascular regulation by the L-arginine metabolites,nitric oxide and agmatine[J]. Pharmacological Research, 2004, 49(5):397-414.

DOI

[25]
ABBAS K, BRETON J, PLANSON A G, et al. Nitric oxide activates an Nrf2/sulfiredoxin antioxidant pathway in macrophages[J]. Free Radical Biology and Medicine, 2011, 51(1):107-114.

DOI PMID

[26]
LORIN J, ZELLER M, GUILLAND J C, et al. Arginine and nitric oxide synthase:regulatory mechanisms and cardiovascular aspects[J]. Molecular Nutrition & Food Research, 2014, 58(1):101-116.

[27]
CAI S, ZHU J L, ZENG X Z, et al. Maternal N-carbamylglutamate supply during early pregnancy enhanced pregnancy outcomes in sows through modulations of targeted genes and metabolism pathways[J]. Journal of Agricultural and Food Chemistry, 2018, 66(23):5845-5852.

DOI PMID

[28]
RENAUDEAU D, COLLIN A, YAHAV S, et al. Adaptation to hot climate and strategies to alleviate heat stress in livestock production[J]. Animal, 2012, 6(5):707-728.

DOI PMID

[29]
QUINIOU N, NOBLET J. Influence of high ambient temperatures on performance of multiparous lactating sows[J]. Journal of Animal Science, 1999, 77(8):2124-2134.

PMID

[30]
WEGNER K, LAMBERTZ C, DAS G, et al. Effects of temperature and temperature-humidity index on the reproductive performance of sows during summer months under a temperate climate[J]. Animal Science Journal, 2016, 87(11):1334-1339.

DOI PMID

[31]
ZHU J L, ZENG X F, PENG Q, et al. Maternal N-carbamylglutamate supplementation during early pregnancy enhances embryonic survival and development through modulation of the endometrial proteome in gilts[J]. The Journal of Nutrition, 2015, 145(10):2212-2220.

[32]
FENG T, BAI J H, XU X L, et al. Supplementation with N-carbamylglutamate and vitamin C:improving gestation and lactation outcomes in sows under heat stress[J]. Animal Production Science, 2017, 58(10):1854-1859.

DOI

[33]
LIU X D, WU X, YIN Y L, et al. Effects of dietary L-arginine or N-carbamylglutamate supplementation during late gestation of sows on the miR-15b/16,miR-221/222,VEGFA and eNOS expression in umbilical vein[J]. Amino Acids, 2012, 42(6):2111-2119.

DOI

[34]
YIN J, REN W, LIU G, et al. Birth oxidative stress and the development of an antioxidant system in newborn piglets[J]. Free Radical Research, 2013, 47(12):1027-1035.

DOI PMID

[35]
UPADHAYA S D, KIM I H. The impact of weaning stress on gut health and the mechanistic aspects of several feed additives contributing to improved gut health function in weanling piglets—a review[J]. Animals, 2021, 11(8):2418.

DOI

[36]
CHE D S, ADAMS S, ZHAO B, et al. Effects of dietary L-arginine supplementation from conception to post- weaning in piglets[J]. Current Protein & Peptide Science, 2019, 20(7):736-749.

[37]
YIN J, REN W K, DUAN J L, et al. Dietary arginine supplementation enhances intestinal expression of SLC7A7 and SLC7A1 and ameliorates growth depression in mycotoxin-challenged pigs[J]. Amino Acids, 2014, 46(4):883-892.

DOI PMID

[38]
ZHANG F R, ZENG X F, YANG F J, et al. Dietary N-carbamylglutamate supplementation boosts intestinal mucosal immunity in Escherichia coli challenged piglets[J]. PLoS One, 2013, 8(6):e66280.

DOI

[39]
WU X, RUAN Z, GAO Y L, et al. Dietary supplementation with L-arginine or N-carbamylglutamate enhances intestinal growth and heat shock protein-70 expression in weanling pigs fed a corn- and soybean meal-based diet[J]. Amino Acids, 2010, 39(3):831-839.

DOI

[40]
YANG H S, FU D Z, KONG X F, et al. Dietary supplementation with N-carbamylglutamate increases the expression of intestinal amino acid transporters in weaned Huanjiang mini-pig piglets[J]. Journal of Animal Science, 2013, 91(6):2740-2748.

DOI

[41]
YI H B, XIONG Y X, WU Q W, et al. Effects of dietary supplementation with L-arginine on the intestinal barrier function in finishing pigs with heat stress[J]. Journal of Animal Physiology and Animal Nutrition, 2020, 104(4):1134-1143.

DOI

[42]
YE C C, ZENG X Z, ZHU J L, et al. Dietary N-carbamylglutamate supplementation in a reduced protein diet affects carcass traits and the profile of muscle amino acids and fatty acids in finishing pigs[J]. Journal of Agricultural and Food Chemistry, 2017, 65(28):5751-5758.

DOI PMID

[43]
XING Y T, WU X, XIE C Y, et al. Meat quality and fatty acid profiles of Chinese Ningxiang pigs following supplementation with N-carbamylglutamate[J]. Animals, 2020, 10(1):88.

DOI

Outlines

/