REVIEW

Research Progress on Regulation of Livestock and Poultry Meat Quality by Niacin

  • MEI Wenliang ,
  • ZHANG Wenyan ,
  • XU Lanjiao ,
  • QU Mingren , *
Expand
  • Engineering Research Center of Nutritional Feed Development, Jiangxi Provincial Key Laboratory of Animal Nutrition, College of Animal Science and Technology, Jiangxi Agricultural University, Nanchang 330045, China
*professor, E-mail:

Received date: 2022-11-02

  Online published: 2023-05-11

Abstract

With the intensive production of livestock and poultry and the enhancement of people’s health awareness, consumers are more and more concerned about the quality and nutritional value of livestock and poultry muscle, such as shear force, drip loss, cooking loss, pH value, intramuscular fat content. Nicotinic acid (NA) is an essential vitamin for animal body to fully synthesize nicotinamide adenine dinucleotide (NAD). It has a variety of biological functions such as antioxidant, lipid metabolism regulation, muscle fiber type conversion promotion, and animal growth performance improvement. This article reviews the effects and possible mechanisms of nicotinic acid in regulating meat quality of livestock and poultry, focusing on the possible mechanisms of nicotinic acid improving meat quality, in order to provide theoretical reference for the application of nicotinic acid in improving meat quality in livestock and poultry production.

Cite this article

MEI Wenliang , ZHANG Wenyan , XU Lanjiao , QU Mingren . Research Progress on Regulation of Livestock and Poultry Meat Quality by Niacin[J]. Chinese Journal of Animal Nutrition, 2023 , 35(5) : 2756 -2764 . DOI: 10.12418/CJAN2023.258

烟酸(NA)是维持动物机体正常生理功能的必需维生素之一,有着广泛的应用前景。烟酸是烟酰胺腺嘌呤二核苷酸(NAD)和烟酰胺腺苷二核苷酸磷酸(NADP)的前体。NAD和NADP参与大多数细胞氧化还原反应,对维持细胞代谢和呼吸至关重要[1]。烟酸在动物体内合成较少,通常无法满足日常消耗,需要在饲粮中进行补充。植物源性烟酸易与肽类、多聚糖形成结合型烟酸,不易于消化,因此动物源性烟酸成为机体补充的主要来源。目前,动物来源饲料不但价格高,而且我国严禁在反刍动物饲粮中使用。因此,如何满足反刍动物对烟酸的需求,充分发挥烟酸作用,成为生产上急需解决的一个问题。
研究表明,烟酸可显著降低大鼠总细胞和核骨髓细胞中的NAD水平[2]。在饲粮中添加烟酸可解决动物源性饲料价格高的问题,还可以缓解畜禽烟酸缺乏带来的生产性能下降,提高断奶仔猪抗炎能力[3]、抗氧化能力[4]、改善肉品质[5]。此外有研究表明,在饲粮中添加烟酸可促进肌内脂肪沉积、改善肉色、提高肌肉品质[6]。本文综述了烟酸对畜禽肉品质的改善作用及其调控机理,为其在畜禽生产中的应用提供理论参考。

1 烟酸的合成代谢与生物学功能

1.1 烟酸的合成与代谢

烟酸又名尼克酸、维生素PP或抗癞皮病因子,是结构最简单的维生素之一。畜禽除了从饲料中获取烟酸,大多数动物都可以利用色氨酸(Trp)和喹啉酸通过犬尿酸途径在肝脏中转化合成烟酸单核苷酸。Trp转化为N-甲酰尿氨酸,N-甲酰尿氨酸转化为α-氨基-β-羧基琥珀酸-ε-半醛(ACMS),ACMS会完全酶氧化或非酶环化,转化为喹啉酸,进而转化为烟酸单核苷酸(NAMN)[7]。NAD生物合成的主要来源是利用膳食烟酸作为前体的补救途径。补救途径包括烟酸磷酸核糖基转移酶(NAPT)催化烟酸转化为NAMN,随后通过烟酰胺单核苷酸腺苷转移酶(NMNAT)和NAD合酶的作用转化为NAD[8-10]。但是,这个过程转化效率很低,受激素、营养、生理病理等多种因素影响,且维生素B6、核黄素、铁和血红素以及维生素B1和Trp的缺乏都会影响转化效率[10]。此外,反刍动物还可以从Trp和喹啉酸中合成烟酸。然而,这种合成效率相对较低,Trp优先用于蛋白质合成。微生物瘤胃合成烟酸被认为是反刍动物烟酸的主要来源[11]
烟酸由胃和小肠吸收,以烟酸和烟酰胺(NAM)的形式进入肝脏,转化为辅酶Ⅰ和辅酶Ⅱ,未经代谢的烟酸和NAM随血液进入其他组织再形成辅酶。过量的烟酸主要经甲基化随尿液排出,其形式有N'-甲基尼克酰胺(NMN)和N-甲基尼克酰胺4-吡啶酮或6-吡啶酮[12-13]

1.2 烟酸的生物学功能

1.2.1 抗炎功能

烟酸可以调节动物机体抗炎能力。研究表明,GPR109A是烟酸的受体,烟酸通过其受体GPR109A控制核因子-κB(NF-κB)向细胞核的移位,来减少巨噬细胞中促炎因子白细胞介素-1β(IL-1β)、肿瘤坏死因子-α(TNF-α)和白细胞介素-6(IL-6)的分泌,减轻机体的炎症反应[14-15]

1.2.2 抗氧化功能

烟酸可提高组织中NAD和NADPH的水平[16],NAD是一种重要的辅酶,参与各种关键的生物过程,也是NAD-依赖性去乙酰化酶(Sirt1)的底物。作为高度保守的去乙酰化酶类,Sirt1已被证明通过激活核因子-红细胞样2相关因子2(Nrf2)途径改善铁过量诱导的氧化应激带来的损伤[17-18]。烟酸显著提高了肺组织中超氧化物歧化酶(SOD)、过氧化氢酶(CAT)活性和谷胱甘肽(GSH)含量[19],此外,烟酸通过下调NF-κB途径,抑制肺组织和血清中的TNF-αIL-6和白细胞介素-8(IL-8)基因表达,减少组织学肺损伤,提高大鼠败血症期间的存活率[20]

1.2.3 调节脂质代谢

烟酸是一种高效的调节高血脂药物,GPR109A对烟酸具有很高的亲和力,烟酸活化GPR109A可以显著降低血液中低密度脂蛋白胆固醇(LDL-C)含量,增加高密度脂蛋白胆固醇(HDL-C)含量[21]。高密度脂蛋白(HDL)具有抗动脉粥样硬化和降低心血管疾病风险的作用[22]。烟酸可增加HDL功能的稳定性,载脂蛋白A-I(ApoA-I)分子常以HDL颗粒相关的脂质形式存在,单独ApoA-I不稳定,容易通过肾脏过滤被清除。烟酸可以通过激活肝脏X受体(LXR)促进膜蛋白ATP结合盒转运体A1(ABCA1)的表达,来调节ApoA-I脂质化和稳定性[23]。烟酸还可降低能引起动脉粥样硬化的所有脂质和脂蛋白颗粒含量,例如,烟酸增加他汀类药物治疗患者HDL中的动脉粥样硬化蛋白含量,包括总胆固醇、甘油三酯、低密度脂蛋白(LDL)[24-25]

1.2.4 促进肌纤维类型转化

根据肌球蛋白重链(MyHC)亚型,肌纤维主要分为MyHC Ⅰ、MyHC Ⅱa、MyHC Ⅱ x和MyHC Ⅱ b 4种类型。且肌纤维类型可以相互转化,受营养和其他因素的影响。Khan等[26]研究发现,在绵羊饲粮中每天添加1 g烟酸可提高过氧化物酶体增殖物激活的受体γ共激活因子β(PGC-1β)和过氧化物酶体增殖物激活的受体γ共激活因子-1α (PGC-1α)的表达,致使肌肉纤维从Ⅱ型过渡到Ⅰ型,从而诱导绵羊骨骼肌的氧化代谢表型;因为烟酸可提高PGC-1α在骨骼肌中的表达水平,它是调节肌肉纤维组成和肌肉代谢表型的关键调节因子。Khan等[5]研究表明,饲粮中添加12 mg/kg烟酸可诱导如PGC-1β和线粒体脂肪酸分解代谢、柠檬酸循环、氧化磷酸化和产热相关基因的表达,促使生长猪Ⅱ型至Ⅰ型肌肉纤维转换。因此,烟酸有促进肌纤维类型转化的作用。

1.2.5 其他功能

烟酸不仅有调节动物机体脂质代谢等功能,还可以调节糖酵解。补充烟酸可提高糖酵解酶甘油醛-3-磷酸脱氢酶的辅助因子氧化型烟酰胺腺嘌呤二核苷酸(NAD+)与还原型烟酰胺腺嘌呤二核苷酸(NADH)的含量[27]。烟酸可以调节细胞中其他能量代谢相关反应,如乳酸脱氢酶的活性和同工酶谱是由烟碱(尼古丁)突触的功能决定的,乳酸脱氢酶催化的乳酸-丙酮酸转化[28]。NAD+和NADH也是线粒体氧化磷酸化的关键介质,它们是线粒体柠檬酸循环中3种限速酶的共同因子,NADH是电子传递链的主要电子供体之一[29];烟酸还可以调节线粒体功能,NAD+/NADH在线粒体柠檬酸循环中起到电子传递链功能,NAD+/NADH还可以调节线粒体通透性转换[30]。NAD+/NADH还可能通过其他机制间接影响线粒体功能,如通过调节影响线粒体活动的钙稳态[31]。此外,烟酸还有延缓机体衰老[32]和提高机体免疫力的功能。

2 烟酸在改善畜禽肉品质上的应用

2.1 烟酸对猪肉品质的影响

猪饲粮中添加不同水平的烟酸,可以促进肌纤维由Ⅱ型转化到Ⅰ型,降低肌肉的蒸煮损失、滴水损失、剪切力,改善肌肉嫩度,提高肌肉的红度和亮度值,降低黄度值,改善肌肉肉色。Khan等[26]在猪饲粮中添加12 mg/kg烟酸,与对照组相比,烟酸组背最长肌、股四头肌、腓肠肌中氧化型肌纤维的百分比升高,而酵解型肌纤维百分比降低,同时调节肌纤维由酵解型向氧化型转化的线粒体脂肪酸分解代谢相关基因——肉碱-酰基肉碱转位酶(CACT)、脂肪酸转运蛋白1(FATP1)、有机阳离子转运蛋白2(OCTN2);柠檬酸循环相关基因——琥珀酸脱氢酶复合体亚单位A(SDHA);氧化磷酸化相关基因——细胞色素c氧化酶亚基4亚型1(COX4/1)和产热相关基因——解偶联蛋白3(UCP3)等关键调节因子在背最长肌中大量表达,提高肌肉的嫩度和多汁性。Real等[33]研究发现,饲粮中添加13、28、55 mg/kg的烟酸均可降低猪背最长肌胴体收缩率和肌肉黄度值,提高持水性,缓解pH24 h的降低,改善肉品质。

2.2 烟酸对家禽肉品质的影响

目前,研究表明饲粮中添加烟酸可以提高家禽胴体品质和生产性能,提高胸肌、腿肌的滴水损失和腿肌pH24 h,改善腿肌嫩度。烟酸还可增加肝脏中ApoA-IApoB和脂联素等脂质代谢相关基因的表达,调节脂质代谢促进肌内脂肪沉积,改善肉品质[34-35]。Zhang等[36]研究表明,在饲粮中添加80 mg/kg烟酸,显著增加五龙鹅胸肌的pH和肌间脂肪宽度,降低胸肌的剪切力、滴水损失和胸肌嫩度,调节血脂水平,提高五龙鹅肉品质。Wu等[37]在饲粮中添加50 mg/kg烟酸和丁酸钠可显著降低高密度饲养下肉鸡胸肌滴水损失和乳酸脱氢酶的活性,增加pH24 h,调节肌肉发育、线粒体生物发生和氧化还原相关基因表达,下调炎症反应、脂质代谢和糖酵解相关基因表达。此外,烟酸还可以调节肌源基因的表达,补充NAM和丁酸钠可以通过上调肌源基因的表达和抑制蛋白质泛素化来改善高放养密度下肉鸡的肉品质,降低肌肉亮度值与滴水损失[38]

2.3 烟酸对反刍动物肉品质的影响

烟酸对反刍动物在肉品质方向的研究较少。研究表明,饲粮中添加烟酸,提高反刍动物生产性能、促进肌纤维类型转化、调节脂质代谢,改善肉品质。Khan等[26]在雄性绵羊饲粮中每天添加1 g烟酸,可显著提高烟酸组骨骼肌的氧化型肌纤维百分比,形成骨骼肌的氧化代谢表型,提高骨骼肌利用脂肪酸的能力。Yang等[6]在育肥牛饲粮中加入1 000 mg/kg烟酸,可增加背最长肌面积、肌内脂肪含量和肌肉红度与亮度值,降低pH24 h和滴水损失,增加血清HDL-C含量,降低了血清LDL-C、甘油三酯、非酯化脂肪酸、总胆固醇的含量,调节脂质代谢,促进肌内脂肪沉积,改善肉品质。

3 烟酸改善畜禽肉品质可能的机制

大量研究表明,烟酸在一定程度上能够改善肉品质,其可能的作用机制总结为以下几点。

3.1 调节机体脂质代谢

研究表明,肌肉内脂肪水平对肉品质至关重要,主要对肌肉的嫩度有着积极的影响[39]。肌内脂肪富含磷脂[40],磷脂内含有大量的多不饱和脂肪酸,在一定程度上改善肌肉的风味。肌内脂肪氧化时可以溶解肌纤维束,在一定程度上可以提高肌肉嫩度和多汁性。烟酸已被证明具有显著的抗血脂作用,可以调节血液中甘油三酯含量,增加HDL-C含量[41-42]
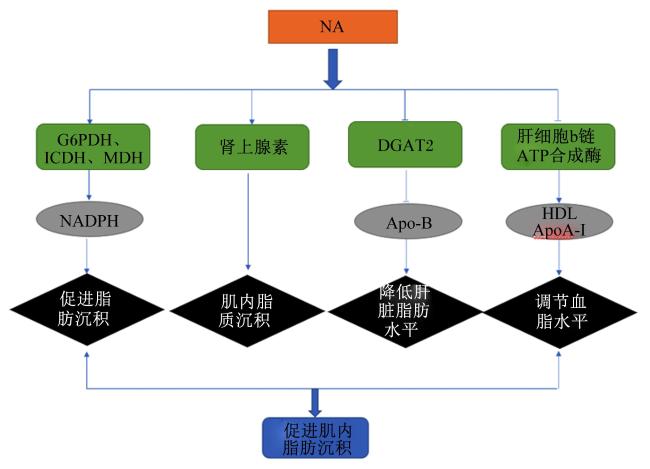
烟酸主要通过影响糖、脂代谢和调节脂代谢相关基因的表达来影响肌内脂肪沉积,烟酸调节机体脂质代谢的机制如图1所示。
图1 烟酸调节机体脂质代谢

NA:烟酸 niacin;G6PDH:葡萄糖-6-磷酸脱氢酶glucose-6-phosphate dehydrogenase; ICDH:异柠檬酸脱氢酶isocitrate dehydrogenase; MDH:苹果酸脱氢酶malate dehydrogenase; NADPH:烟酰胺腺嘌呤二核苷酸磷酸(还原态)nicotinamide adenine dinucleotide phosphate (reduced state); DGAT2:二酰基甘油酰基转移酶2 diacylglycerol acyltransferase 2; ApoA-I:载脂蛋白A-I apolipoprotein A-I; Apo-B:载脂蛋白B apolipoprotein-B; HDL:高密度脂蛋白 high-density lipoprotein。

Fig.1 Niacin regulates lipid metabolism in body

NADPH是调节脂肪酸合成最重要的酶之一[43],NADPH合成需要葡萄糖-6-磷酸脱氢酶(G6PD)、苹果酸脱氢酶(MDH)和异柠檬酸脱氢酶(ICDH)的参与[44]。添加烟酸可提高背最长肌中G6PDH、ICDH和MDH活性以及NADPH水平,导致脂肪酸从头合成,促进脂肪沉积[6]。此外,烟酸通过下调脂肪细胞中CCAAT增强子结合蛋白β(CCAAT enhancer binding proteins, C/EBPβ)激活的环氧合酶-2表达来抑制抗脂肪PGF(2α)的产生,从而促进脂肪生成[45]。烟酸选择性抑制肝脏二酰基甘油酰基转移酶2(DGAT2)mRNA表达和微粒体活性[46],DGAT2是催化甘油三酯合成的关键酶,烟酸直接抑制人肝细胞DGAT2,导致肝脏Apo-B降解加速和Apo-B分泌减少,显著降低肝脏脂肪水平[47-48]。HDL含有的ApoA-I是胆固醇逆向转运的主要参与者,它们将外周组织多余的胆固醇运至肝脏加工或降解[49]。烟酸通过降低肝脏表面肝细胞b链ATP合成酶的表达,减少肝脏对HDL ApoA-I的分解代谢[50],提高循环中HDL ApoA-I水平,调节血脂水平。综上所述,烟酸可以调节机体脂代谢相关基因的表达和影响糖、脂代谢,促进肌内脂肪沉积,改善肉品质。

3.2 提高机体抗氧化能力

随着动物集约化饲养,畜禽更容易受到氧化应激的损伤。氧化应激对肌肉的影响主要是导致与肌肉嫩度相关的蛋白水解酶失活和肌肉蛋白氧化使蛋白水解度降低[51-52]。蛋白质氧化会降低其蛋白质溶解度,增加肌肉的滴水损失[53]。脂质氧化和肌红蛋白氧化会导致肉类异味和变色[54]
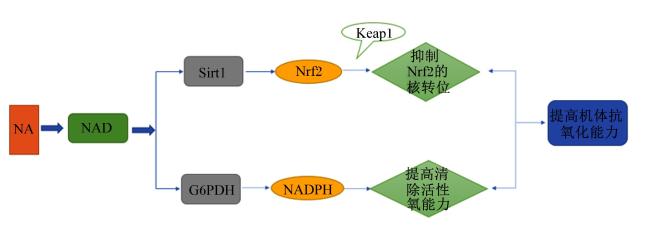
烟酸提高机体抗氧化能力的机制如图2所示。目前,已证实烟酸具有减轻慢性肾衰竭大鼠模型中氧化应激的作用[55],且烟酸可以通过调节活性氧依赖性NF-κB通路,改善急性肺损伤[19]。烟酸作为NAD和NADP的前体,口服烟酸可提高肝脏中NAD的水平[16]。NAD是一种重要的辅酶,参与各种关键的生物过程,是Sirt1的底物。作为一种III类组蛋白脱乙酰酶,Sirt1通过激活Nrf2[17],Nrf2调节下游抗氧化酶血红素加氧酶-1(HO-1)和NADPH醌氧化还原酶-1(NQO-1)的表达,减轻活性氧造成的损伤[56-57]。NAD上调葡萄糖-6-磷酸脱氢酶的表达,葡萄糖-6-磷酸脱氢酶是限速酶,可调节NADPH的合成。NADPH是细胞抗氧化系统的关键成分[29]。NADPH还通过调节谷胱甘肽还原酶活性促进还原型谷胱甘肽生成。还原型谷胱甘肽是一种重要的抗氧化剂。在烟酸存在下,MDA和共轭二烯的浓度较低,还原型谷胱甘肽和维生素E的水平较高,还原型谷胱甘肽也参与维生素E的再生,维生素E是另一种重要的膜抗氧化剂[58]。综上所述,烟酸可以调节机体抗氧化相关基因的表达和抗氧化酶活性,提高机体抗氧化能力,改善肉品质。
图2 烟酸提高机体抗氧化能力

Nrf2:核因子-红细胞样2相关因子2 nuclear factor-erythroid-like 2-related factor 2; G6PDH;葡萄糖-6-磷酸脱氢酶glucose-6-phosphate dehydrogenase; NAD:烟酰胺腺嘌呤二核苷酸nicotinamide adenine dinucleotide; NA:烟酸niacin; Sirt1:NAD-依赖性去乙酰化酶 NAD-dependent deacetylase。

Fig.2 Niacin increases antioxidant capacity in body

3.3 促进肌纤维类型转化

肌纤维占肌肉体积的75%~90%。纤维类型组成影响肌肉代谢特性,不同的肌纤维类型代谢酶活性、蛋白质和脂肪含量存在差异,对肉品质起关键作用。研究表明,氧化型肌纤维中肌红蛋白含量高,与氧结合后呈现鲜红色。肌肉中氧化型肌纤维比例高时,肌肉色泽更加鲜红[59]。Ⅰ型肌纤维数目占比与肉品质密切相关,与剪切力呈负相关[60]。Ⅱ型肌纤维代谢类型主要是无氧酵解,当其比例增高,pH24 h相对于Ⅰ型肌纤维下降更快。
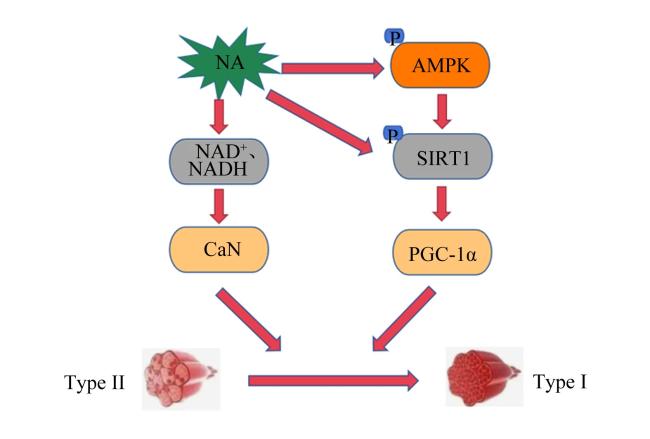
烟酸促进肌纤维类型转化的机制如图3所示。研究表明,烟酸可能通过AMPK/Sirt1/PGC-1ɑ和钙离子(Ca2+)信号通路调节骨骼肌纤维类型转化,改善肉品质。AMPK、Sirt1和PGC-1ɑ在调节线粒体能量代谢[61]和骨骼肌纤维类型转换[62]中发挥关键作用。小鼠骨骼肌训练与磷酸化AMPK(P-AMPK)活性密切相关,小鼠骨骼肌训练增加可促进P-AMPK表达,且增加氧化型肌纤维的比例[63]。5-氨基咪唑-4-甲酰胺-1-β-D-核糖醛苷(AICAR)是AMPK的激活剂,大鼠皮下注射AICAR可增加大鼠骨骼肌中Ⅱx型肌纤维的比例[64]。PGC-1α和PGC-1β通过调节肌肉纤维分布和骨骼肌代谢表型促进肌纤维转化,补充烟酸可增加肌纤维类型转化关键调节因子PGC-1αPGC-1β的表达[26]。Sirt1是一类依赖NAD+的去乙酰化酶,NAD+是Sirt1的底物,Sirt1/PGC-1ɑ可调节骨骼肌纤维类型转换[62],提高氧化型肌纤维的比例,改善肉品质。
图3 烟酸促进肌纤维类型转化

NA:烟酸niacin; NAD+:烟酰胺腺嘌呤二核苷酸(氧化态)nicotinamide adenine dinucleotide (oxidized state); NADH:烟酰胺腺嘌呤二核苷酸(还原态)nicotinamide adenine dinucleotide (reduced state); CaN:钙调磷酸酶calcium-regulated phosphatase; AMPK:腺苷酸激活蛋白激酶adenylate-activated protein kinase; PGC-1α:过氧化物酶体增殖物激活的受体γ共激活因子-1α peroxisome proliferator-activated receptor gamma co-activator-1α; Sirt1:NAD-依赖性去乙酰化酶NAD-dependent deacetylase。

Fig.3 Niacin promotes muscle fibre type conversion

NAD+和NADH可调节钙稳态使Ca2+内流[29]。钙调磷酸酶-活化T细胞(NFAT)是调节骨骼肌纤维类型转化的重要通路,Ca2+可激活钙调磷酸酶(Cn),其由通过钙调磷酸酶A(CnA)催化亚基和钙调磷酸酶B(CnB)调节亚基的结合形成的异二聚体组成。CnA通过去磷酸化刺激NFAT转录因子的核因子活性[65]。NFAT是Cn的主要靶标[66]。研究表明,小鼠骨骼肌中Cn过表达可提高氧化型肌纤维比例[67],而敲除Cn的小鼠,骨骼肌氧化型肌纤维比例下降[68]。综上所述,CaN/NFAT途径可促进酵解型肌纤维转化为氧化型肌纤维。
钙调蛋白依赖性蛋白激酶(CAMKs)/组蛋白去乙酰化酶4(HDAC4)/肌细胞增强因子2(Mef2)是另一条通过Ca2+促进肌纤维类型转化的途径。CaMKs调节HDAC4去磷酸化并激活Mef2,调节骨骼肌纤维类型的转化[69]。综上所述,烟酸可以通过调节机体肌纤维类型转换关键基因的表达而改变肌肉的代谢表型,达到改善肉品质的效果。

4 小结

烟酸作为一种饲料添加剂,具有抗炎、抗氧化、调节脂质代谢和糖酵解、调控细胞能量状态、促进肌纤维类型转化等生理功能。本文从烟酸调节脂质代谢、抗氧化及调节肌纤维类型转化,并从烟酸及其受体等多条信号通路综述其影响肉品质的作用机制,为烟酸调节畜禽肉品质提供了参考资料。目前,关于烟酸的功能及其对肉品质的影响引起密切的关注和研究,但仍有许多问题值得进一步研究,包括烟酸调控不同部位脂代谢的作用机制、烟酸调控能量代谢以及烟酸通过调控肠道菌群对肉品质的影响等。烟酸调控肉品质机制十分复杂,深入探明烟酸对肉品质影响的分子机制仍是今后研究的重点。
[1]
KIRKLAND J B, MEYER-FICCA M L. Niacin[J]. Advances in Food and Nutrition Research, 2018, 83:83-149.

DOI PMID

[2]
TANG K, SHAM H, HUI E, et al. Niacin deficiency causes oxidative stress in rat bone marrow cells but not through decreased NADPH or glutathione status[J]. The Journal of Nutritional Biochemistry, 2008, 19(11):746-753.

DOI

[3]
FENG J S, WANG L, CHEN Y B, et al. Effects of niacin on intestinal immunity,microbial community and intestinal barrier in weaned piglets during starvation[J]. International Immunopharmacology, 2021, 95:107584.

DOI

[4]
段晨磊, 王宝维, 葛文华, 等. 烟酸对五龙鹅抗氧化性能和免疫性能的影响[J]. 中国畜牧杂志, 2016, 52(1):32-37.

DUAN C L, WANG B W, GE W H, et al. Effects of different dietary level of nicotinic acid on anti-oxidation and immunity of Wulong geese[J]. Chinese Journal of Animal Science, 2016, 52(1):32-37. (in Chinese)

[5]
KHAN M, RINGSEIS R, MOOREN F C, et al. Niacin supplementation increases the number of oxidative type Ⅰ fibers in skeletal muscle of growing pigs[J]. BMC Veterinary Research, 2013, 9:177.

DOI

[6]
YANG Z Q, BAO L B, ZHAO X H, et al. Nicotinic acid supplementation in diet favored intramuscular fat deposition and lipid metabolism in finishing steers[J]. Experimental Biology and Medicine, 2016, 241(11):1195-1201.

DOI

[7]
SRIVASTAVA S. Emerging therapeutic roles for NAD+ metabolism in mitochondrial and age-related disorders[J]. Clinical and Translational Medicine, 2016, 5(1):e25.

[8]
CANTÓ C, MENZIES K J, AUWERX J. NAD+ metabolism and the control of energy homeostasis:a balancing act between mitochondria and the nucleus[J]. Cell Metabolism, 2015, 22(1):31-53.

DOI

[9]
HOUTKOOPER R H, CANTÓ C, WANDERS R J, et al. The secret life of NAD+:an old metabolite controlling new metabolic signaling pathways[J]. Endocrine Reviews, 2010, 31(2):194-223.

DOI

[10]
GASPERI V, SIBILANO M, SAVINI I, et al. Niacin in the central nervous system:an update of biological aspects and clinical applications[J]. International Journal of Molecular Sciences, 2019, 20(4):974.

DOI

[11]
CHEN J, YANG Z, DONG G. Niacin nutrition and rumen-protected niacin supplementation in dairy cows:an updated review[J]. The British Journal of Nutrition, 2019, 122(10):1103-1112.

DOI

[12]
龙凡, 梅文亮, 许兰娇, 等. 烟酸的生物学功能及其在畜禽生产中的应用[J]. 动物营养学报, 2022, 34(7):4143-4154.

DOI

LONG F, MEI W L, XU L J, et al. Biological functions of niacin and its application in livestock and poultry production[J]. Chinese Journal of Animal Nutrition, 2022, 34(7):4143-4154. (in Chinese)

DOI

[13]
邹必成, 龙凡, 瞿明仁, 等. 烟酸缓解反刍动物热应激的研究进展[J]. 动物营养学报, 2022, 34(4):2130-2139.

DOI

ZOU B C, LONG F, QU M R, et al. Research progress of niacin to relieve heat stress in ruminants[J]. Chinese Journal of Animal Nutrition, 2022, 34(4):2130-2139. (in Chinese)

[14]
GIRI B, BELANGER K, SEAMON M, et al. Niacin ameliorates neuro-inflammation in Parkinson’s disease via GPR109A[J]. International Journal of Molecular Sciences, 2019, 20(18):4559.

DOI

[15]
FENG L, LI S Q, JIANG W D, et al. Deficiency of dietary niacin impaired intestinal mucosal immune function via regulating intestinal NF-κB,Nrf2 and MLCK signaling pathways in young grass carp (Ctenopharyngodon idella)[J]. Fish & Shellfish Immunology, 2016, 49:177-193.

[16]
LI Q, XIE G X, ZHANG W L, et al. Dietary nicotinic acid supplementation ameliorates chronic alcohol-induced fatty liver in rats[J]. Alcohol:Clinical and Experimental Research, 2014, 38(7):1982-1992.

DOI

[17]
DA CUNHA M D S B, ARRUDA S F. Tucum-do-cerrado (Bactris setosa Mart.) may promote anti-aging effect by upregulating SIRT1-Nrf2 pathway and attenuating oxidative stress and inflammation[J]. Nutrients, 2017, 9(11):1243.

DOI

[18]
HU D, ZHANG L, JIANG R, et al. Nicotinic acid against acetaminophen-induced hepatotoxicity via Sirt1/Nrf2 antioxidative pathway in mice[J]. Journal of Nutritional Science and Vitaminology, 2021, 67(3):145-152.

DOI PMID

[19]
JEONG K Y, SUH G J, KWON W Y, et al. The therapeutic effect and mechanism of niacin on acute lung injury in a rat model of hemorrhagic shock:down-regulation of the reactive oxygen species-dependent nuclear factor κB pathway[J]. The Journal of Trauma and Acute Care Surgery, 2015, 79(2):247-255.

DOI

[20]
KWON W Y, SUH G J, KIM K S, et al. Niacin attenuates lung inflammation and improves survival during sepsis by downregulating the nuclear factor-κB pathway[J]. Critical Care Medicine, 2011, 39(2):328-334.

DOI PMID

[21]
KOTHAWADE P B, THOMAS A B, CHITLANGE S S. Novel niacin receptor agonists:a promising strategy for the treatment of dyslipidemia[J]. Mini Reviews in Medicinal Chemistry, 2021, 21(17):2481-2496.

DOI

[22]
ERTEK S. High-density Lipoprotein (HDL) dysfunction and the future of HDL[J]. Current Vascular Pharmacology, 2018, 16(5):490-498.

DOI PMID

[23]
ZHANG L H, KAMANNA V S, GANJI S H, et al. Niacin increases HDL biogenesis by enhancing Dr4-dependent transcription of ABCA1 and lipidation of apolipoprotein A-I in HepG2 cells[J]. Journal of Lipid Research, 2012, 53(5):941-950.

DOI

[24]
RONSEIN G E, VAISAR T, DAVIDSON W S, et al. Niacin increases atherogenic proteins in high-density lipoprotein of statin-treated subjects[J]. Arteriosclerosis,Thrombosis,and Vascular Biology, 2021, 41(8):2330-2341.

DOI

[25]
FEINGOLD K R. Triglyceride lowering drugs[M]//FEINGOLD K R,ANAWALT B,BLACKMAN M R,et al. Endotext [Internet].South Dartmouth (MA): MDText. com,Inc., 2000:NBK425699.

[26]
KHAN M, COUTURIER A, KUBENS J F, et al. Niacin supplementation induces type Ⅱ to type Ⅰ muscle fiber transition in skeletal muscle of sheep[J]. Acta Veterinaria Scandinavica, 2013, 55(1):85.

DOI

[27]
PIRINEN E, AURANEN M, KHAN N A, et al. Niacin cures systemic NAD+ deficiency and improves muscle performance in adult-onset mitochondrial myopathy[J]. Cell Metabolism, 2020, 31(6):1078-1090.e5.

DOI

[28]
FARHANA A, LAPPIN S L. Biochemistry,lactate dehydrogenase[M/OL]// Anon.StatPearls [Internet]. Treasure Island: StatPearls Publishing, 2022:NBK557536.[2023-02-21]. https://pubmed.ncbi.nlm.nih.gov/32491468/.

[29]
YING W H. NAD+/NADH and NADP+/NADPH in cellular functions and cell death:regulation and biological consequences[J]. Antioxidants & Redox Signaling, 2008, 10(2):179-206.

[30]
ROTTENBERG H, HOEK J B. The mitochondrial permeability transition:nexus of aging,disease and longevity[J]. Cells, 2021, 10(1):79.

DOI

[31]
NICHOLLS D G, BUDD S L, WARD M W, et al. Excitotoxicity and mitochondria[J]. Biochemical Society Symposium, 1999, 66:55-67.

PMID

[32]
SHARMA R, RAMANATHAN A. The aging metabolome-biomarkers to hub metabolites[J]. Proteomics, 2020, 20(5/6):e1800407.

[33]
REAL D E, NELSSEN J L, UNRUH J A, et al. Effects of increasing dietary niacin on growth performance and meat quality in finishing pigs reared in two different environments[J]. Journal of Animal Science, 2002, 80(12):3203-3210.

PMID

[34]
JIANG R R, ZHAO G P, ZHAO J P, et al. Influence of dietary nicotinic acid supplementation on lipid metabolism and related gene expression in two distinct broiler breeds of female chickens[J]. Journal of Animal Physiology and Animal Nutrition, 2014, 98(5):822-829.

PMID

[35]
JIANG R R, ZHAO G P, CHEN J L, et al. Effect of dietary supplemental nicotinic acid on growth performance,carcass characteristics and meat quality in three genotypes of chicken[J]. Journal of Animal Physiology and Animal Nutrition, 2011, 95(2):137-145.

DOI

[36]
ZHANG B B, HAO J Z, YIN H J, et al. Effects of dietary nicotinic acid supplementation on meat quality,carcass characteristics,lipid metabolism,and tibia parameters of Wulong geese[J]. Poultry Science, 2021, 100(11):101430.

DOI

[37]
WU Y Q, WANG Y L, YIN D F, et al. Transcriptome analysis reveals a molecular understanding of nicotinamide and butyrate sodium on meat quality of broilers under high stocking density[J]. BMC Genomics, 2020, 21(1):412.

DOI PMID

[38]
WU Y Q, WANG Y L, WU W, et al. Effects of nicotinamide and sodium butyrate on meat quality and muscle ubiquitination degradation genes in broilers reared at a high stocking density[J]. Poultry Science, 2020, 99(3):1462-1470.

DOI PMID

[39]
ZHAO X H, YANG Z Q, BAO L B, et al. Daidzein enhances intramuscular fat deposition and improves meat quality in finishing steers[J]. Experimental Biology and Medicine, 2015, 240(9):1152-1157.

DOI

[40]
THOMAS E M, RODEN J A, HARESIGN W, et al. Meat eating and nutritional quality of lambs sired by high and low muscle density rams[J]. Animal, 2021, 15(3):100136.

DOI

[41]
GORDON S M, AMAR M J, JEIRAN K, et al. Effect of niacin monotherapy on high density lipoprotein composition and function[J]. Lipids in Health and Disease, 2020, 19(1):190.

DOI PMID

[42]
LA PAZ S M D, BERMUDEZ B, NARANJO M C, et al. Pharmacological effects of niacin on acute hyperlipemia[J]. Current Medicinal Chemistry, 2016, 23(25):2826-2835.

DOI

[43]
ZHANG Z Y, TESLAA T, XU X C, et al. Serine catabolism generates liver NADPH and supports hepatic lipogenesis[J]. Nature Metabolism, 2021, 3(12):1608-1620.

DOI PMID

[44]
FREDERIKS W M, KÜMMERLIN I P E D, BOSCH K S, et al. NADPH production by the pentose phosphate pathway in the zona fasciculata of rat adrenal gland[J]. Journal of Histochemistry & Cytochemistry, 2007, 55(9):975-980.

DOI

[45]
FUJIMORI K, AMANO F. Niacin promotes adipogenesis by reducing production of anti-adipogenic PGF through suppression of C/EBPβ-activated COX-2 expression[J]. Prostaglandins & Other Lipid Mediators, 2011, 94(3/4):96-103.

[46]
GANJI S H, TAVINTHARAN S, ZHU D M, et al. Niacin noncompetitively inhibits DGAT2 but not DGAT1 activity in HepG2 cells[J]. Journal of Lipid Research, 2004, 45(10):1835-1845.

DOI PMID

[47]
KAMANNA V S, KASHYAP M L. Nicotinic acid (niacin) receptor agonists:will they be useful therapeutic agents?[J]. The American Journal of Cardiology, 2007, 100(<W>11 A):S53-S61.

[48]
HU M, CHU W C W, YAMASHITA S, et al. Liver fat reduction with niacin is influenced by DGAT-2 polymorphisms in hypertriglyceridemic patients[J]. Journal of Lipid Research, 2012, 53(4):802-809.

DOI

[49]
VAN DER VORST E P C. High-density lipoproteins and apolipoprotein A1[J]. Sub-cellular Biochemistry, 2020, 94:399-420.

DOI PMID

[50]
ZHANG L H, KAMANNA V S, ZHANG M C, et al. Niacin inhibits surface expression of ATP synthase β chain in HepG2 cells:implications for raising HDL[J]. Journal of Lipid Research, 2008, 49(6):1195-1201.

DOI

[51]
HUFF LONERGAN E, ZHANG W G, LONERGAN S M. Biochemistry of postmortem muscle-lessons on mechanisms of meat tenderization[J]. Meat Science, 2010, 86(1):184-195.

DOI

[52]
CARLIN K R M, HUFF-LONERGAN E, ROWE L J, et al. Effect of oxidation,pH,and ionic strength on calpastatin inhibition of mu- and m-calpain[J]. Journal of Animal Science, 2006, 84(4):925-937.

DOI

[53]
WANG R R, PAN X J, PENG Z Q. Effects of heat exposure on muscle oxidation and protein functionalities of pectoralis majors in broilers[J]. Poultry Science, 2009, 88(5):1078-1084.

DOI PMID

[54]
FAUSTMAN C, SUN Q, MANCINI R, et al. Myoglobin and lipid oxidation interactions:mechanistic bases and control[J]. Meat Science, 2010, 86(1):86-94.

DOI

[55]
CHO K H, KIM H J, RODRIGUEZ-ITURBE B, et al. Niacin ameliorates oxidative stress,inflammation,proteinuria,and hypertension in rats with chronic renal failure[J]. American Journal of Physiology. Renal Physiology, 2009, 297(1):F106-F113.

DOI

[56]
ZHAO Y, SUN Y Z, WANG G Y, et al. Dendrobium officinale polysaccharides protect against MNNG-induced PLGC in rats via activating the NRF2 and antioxidant enzymes HO-1 and NQO-1[J]. Oxidative Medicine and Cellular Longevity, 2019, 2019:9310245.

[57]
LOU Y M, GUO Z Z, ZHU Y F, et al. Houttuynia cordata Thunb. and its bioactive compound 2-undecanone significantly suppress benzo(a)pyrene-induced lung tumorigenesis by activating the Nrf2-HO-1/NQO-1 signaling pathway[J]. Journal of Experimental & Clinical Cancer Research, 2019, 38(1):242.

[58]
ARUN P, PADMAKUMARAN NAIR K G, MANOJKUMAR V, et al. Decreased hemolysis and lipid peroxidation in blood during storage in the presence of nicotinic acid[J]. Vox Sanguinis, 1999, 76(4):220-225.

PMID

[59]
MATARNEH S K, SILVA S L, GERRARD D E. New insights in muscle biology that alter meat quality[J]. Annual Review of Animal Biosciences, 2021, 9:355-377.

DOI PMID

[60]
杨玉莹, 张一敏, 毛衍伟, 等. 不同部位牦牛肉肌纤维特性与肉品质差异[J]. 食品科学, 2019, 40(21):72-77.

DOI

YANG Y Y, ZHANG Y M, MAO Y W, et al. Differences in myofiber characteristics and meat quality of different yak muscles[J]. Food Science, 2019, 40(21):72-77. (in Chinese)

DOI

[61]
TIAN L, CAO W J, YUE R J, et al. Pretreatment with Tilianin improves mitochondrial energy metabolism and oxidative stress in rats with myocardial ischemia/reperfusion injury via AMPK/SIRT1/PGC-1 alpha signaling pathway[J]. Journal of Pharmacological Sciences, 2019, 139(4):352-360.

DOI PMID

[62]
WEN W X, CHEN X L, HUANG Z Q, et al. miR-22-3p regulates muscle fiber-type conversion through inhibiting AMPK/SIRT1/PGC-1α pathway[J]. Animal Biotechnology, 2021, 32(2):254-261.

DOI

[63]
RÖCKL K S C, HIRSHMAN M F, BRANDAUER J, et al. Skeletal muscle adaptation to exercise training:AMP-activated protein kinase mediates muscle fiber type shift[J]. Diabetes, 2007, 56(8):2062-2069.

DOI

[64]
SUWA M, NAKANO H, KUMAGAI S. Effects of chronic AICAR treatment on fiber composition,enzyme activity,UCP3,and PGC-1 in rat muscles[J]. Journal of Applied Physiology, 2003, 95(3):960-968.

DOI

[65]
LUO P, WANG L N, LUO L, et al. Ca2+-calcineurin-NFAT pathway mediates the effect of thymol on oxidative metabolism and fiber-type switch in skeletal muscle[J]. Food & Function, 2019, 10(8):5166-5173.

[66]
MCCULLAGH K J A, CALABRIA E, PALLAFACCHINA G, et al. NFAT is a nerve activity sensor in skeletal muscle and controls activity-dependent myosin switching[J]. Proceedings of the National Academy of Sciences of the United States of America, 2004, 101(29):10590-10595.

PMID

[67]
NAYA F J, MERCER B, SHELTON J, et al. Stimulation of slow skeletal muscle fiber gene expression by calcineurin in vivo[J]. Journal of Biological Chemistry, 2000, 275(7):4545-4548.

DOI

[68]
PARSONS S A, MILLAY D P, WILKINS B J, et al. Genetic loss of calcineurin blocks mechanical overload-induced skeletal muscle fiber type switching but not hypertrophy[J]. Journal of Biological Chemistry, 2004, 279(25):26192-26200.

DOI PMID

[69]
COHEN T J, CHOI M C, KAPUR M, et al. HDAC4 regulates muscle fiber type-specific gene expression programs[J]. Molecules and Cells, 2015, 38(4):343-348.

DOI PMID

Outlines

/