RESEARCH PAPER

Effects of Porcine Lactobacillus reuteri LR1 on Growth Performance and Intestinal Epithelial Barrier Function of Piglets at 42 Days after Weaning

  • LIU Chunyan , 1, 2 ,
  • SUN Yanjie 1 ,
  • WANG Qian 1 ,
  • XIONG Yunxia 2 ,
  • WU Qiwen 2 ,
  • YANG Xuefen 2 ,
  • WANG Li 2 ,
  • JIANG Zongyong 2 ,
  • YI Hongbo , 2, * ,
  • HUANG Yanna , 1, *
Expand
  • 1 College of Animal Science and Technology, Guangxi University, Nanning 530004, China
  • 2 Guangdong Key Laboratory of Animal Breeding and Nutrition, Maoming Branch of Guangdong Laboratory for Lingnan Modern Agriculture, Key Laboratory of Animal Nutrition and Feed Science in South China, Ministry of Agriculture and Rural Affairs, State Key Laboratory of Livestock and Poultry Breeding, Institute of Animal Science, Guangdong Academy of Agricultural Sciences, Guangzhou 510640, China
*YI Hongbo, associate professor, E-mail: ;
HUANG Yanna, associate professor, E-mail:

Received date: 2022-12-07

  Online published: 2023-06-08

Abstract

This experiment was conducted to investigate the effects of porcine Lactobacillus reuteri LR1 on growth performance and intestinal epithelial barrier function of piglets at 42 days after weaning. A total of 144 weaned Duroc crossbred piglets with similar body weight at 21 days of age were randomly divided into 3 groups, which were fed a basal diet (control group, CON group), the basal diet supplemented with 75 mg/kg aureamycin and 100 mg/kg quinolindox (antibiotic group, AO group) and the basal diet was supplemented with 5×10¹⁰ CFU/kg Lactobacillus reuteri LR1 (Lactobacillus reuteri group, LR1 group) with 8 replicates per group and 6 piglets per replicate (half male and half female). The experiment lasted for 42 days. The results showed as follows: 1) compared with CON group, the average daily gain in LR1 group was significantly increased (P<0.05). 2) Compared with CON group, LR1 increased the villus height of duodenum, jejunum and ileum (P<0.05), and increased the ratio of villus to crypt of duodenum and ileum (P<0.05). 3) Compared with CON group, the gene relative expression levels of colonic ZO-1 and Occludin in LR1 group was significantly increased (P<0.05). 4) Compared with CON group, the gene relative expression level of mucin-2 (MUC-2) in jejunum in LR1 group was significantly increased (P<0.05), and the gene relative expression levels of MUC-1 and MUC-2 in colon were significantly increased (P<0.05). 5) Compared with CON group, the relative gene expression level of porcine β-defansin 3 (pBD3) in ileum LR1 group was significantly increased (P<0.05), and the gene relative expression levels of pBD2 and pBD3 in colon were significantly increased (P<0.05). 6) Compared with CON group, the colonic Toll-like receptor-2 (TLR2) gene relative expression level in LR1 group was significantly increased (P<0.05). It is concluded that dietary Lactobacillus reuteri LR1 can improve the growth performance of piglets at 42 days after weaning, improve the intestinal villus morphology, significantly increase the expressions of colon-intestinal tight junction protein, mucin, antimicrobial peptides and Toll-like receptor genes, and thus improve the intestinal epithelial barrier function of weaned piglets.

Cite this article

LIU Chunyan , SUN Yanjie , WANG Qian , XIONG Yunxia , WU Qiwen , YANG Xuefen , WANG Li , JIANG Zongyong , YI Hongbo , HUANG Yanna . Effects of Porcine Lactobacillus reuteri LR1 on Growth Performance and Intestinal Epithelial Barrier Function of Piglets at 42 Days after Weaning[J]. Chinese Journal of Animal Nutrition, 2023 , 35(6) : 3583 -3593 . DOI: 10.12418/CJAN2023.334

仔猪断奶应激易造成肠道上皮屏障功能损伤,易引发严重腹泻。在过去的几十年,抗生素和氧化锌是预防治疗仔猪断奶应激的有效添加剂,但过度使用会造成一定的耐药性已经对环境产生副作用,因此我国目前已对饲料添加剂采取禁抗、限锌的措施,生猪养殖从业者面临巨大困扰。罗伊氏乳杆菌(Lactobacillus reuteri,LR)是一种天然定植在哺乳动物和鸟类肠道的益生菌,在维持动物健康和免疫调节等方面有着重要意义[1],已被证明可以调节先天免疫反应和肠道屏障功能[2-3]。先前对小鼠的研究表明,LR可通过上调紧密连接蛋白(tight junction protein,TJ)的表达来改善肠道屏障功能[4],此外,LR I5007也可通过脂多糖刺激猪小肠上皮细胞和新生仔猪分泌TJ来增强新生猪的肠道屏障功能[5]。同时,Liu等[3]研究发现,喂养健康新生小鼠LR DSM 17938可调节免疫反应,同时调节肠道微生物群并促进有益代谢物的产生。此前,本课题组从健康断奶仔猪的粪便中分离出新型猪源LR1,并发现LR1可以提高断奶后14 d仔猪生长性能并改善肠上皮屏障功能以缓解仔猪的腹泻[6-8]。同时,我们利用猪小肠上皮细胞研究LR1如何影响产肠毒素大肠杆菌K88诱导的肠道损伤,结果显示LR1可以通过抑制肌球蛋白轻链激酶信号通路来抑制产肠毒素大肠杆菌K88诱导的炎症反应[9]。然而,很少关注LR1对断奶后42 d仔猪肠道上皮屏障功能的影响,因此,本试验旨在研究LR1对断奶后42 d仔猪的生长性能、肠道形态以及肠道上皮屏障功能等方面的影响,以期为LR1在仔猪生产中的应用提供理论依据。

1 材料与方法

1.1 试验方法

选取144头21日龄杜长大杂交断奶仔猪,随机分为3组,每组8个重复,每个重复6头仔猪,公母各占1/2,每栏之间的体重接近(P>0.05)。对照组(CON组)饲喂基础饲粮,其参照NRC(2012)营养需要配制成粉状配合饲料,表1为基础饲粮组成及营养水平。试验组分为抗生素组(AO组)和LR1组,分别在基础饲粮中添加75 mg/kg金霉素和100 mg/kg喹乙醇、猪源LR1(5×1010 CFU/kg,根据Yang等[10]的报道确定添加量)。益生菌制剂经喷雾干燥制成冻干粉,饲喂前经逐级稀释与粉状饲料混合均匀。试验期42 d。仔猪自由采食,充足饮水,所有猪只均按正常免疫程序进行免疫接种。
表1 基础饲粮组成及营养水平(风干基础)

Table 1 Composition and nutrient levels of basal diets (air-dry basis)%

项目
Items
含量 Content
1~14 d 15~42 d
原料 Ingredients
玉米 Corn 35.31 47.55
膨化玉米 Extruded corn 15.00 13.00
发酵豆粕 Fermented soybean meal 9.00 8.50
去皮大豆粕 Dehulled soybean meal 9.00
膨化大豆 Extruded soybean 10.00 6.00
鱼粉 Fish meal 4.00 4.00
乳清粉 Dried whey 11.00 6.00
大豆皮 Soybean hull 5.00
大豆油 Soybean oil 1.20
浓缩乳清蛋白 Whey protein concentrate 3.00
白砂糖 Custer sugar 2.00 2.00
50%氯化胆碱 50% choline chloride 0.20 0.18
食盐 NaCl 0.45 0.45
磷酸氢钙 CaHPO4 0.62 0.60
石粉 Limestone 0.65 0.74
L-赖氨酸盐酸盐 L-Lys·HCl 0.60 0.54
DL-蛋氨酸 DL-Met 0.22 0.20
L-苏氨酸 L-Thr 0.21 0.21
L-色氨酸 L-Try 0.04 0.03
预混料 Premix1) 1.50 1.00
合计 Total 100.00 100.00
营养水平 Nutrient levels2)
消化能 DE/(MJ/kg) 14.85 14.71
粗蛋白质 CP 19.20 19.10
钙 Ca 0.68 0.70
总磷 TP 0.56 0.53
标准全消化道可消化磷 STTDP 0.40 0.34
标准回肠可消化赖氨酸 SID Lys 1.42 1.29
标准回肠可消化蛋氨酸+标准回肠可消化半胱氨酸
SID Met+ SID Cys
0.57 0.54
标准回肠可消化苏氨酸 SID Thr 0.85 0.80
标准回肠可消化色氨酸 SID Try 0.24 0.21

1)预混料中含多维400 mg/kg、多矿2 000 mg/kg,其具体组成见参考文献[11]。

2)粗蛋白质、钙、总磷为实测值,其余为计算值。

1)The premix contained 400 mg/kg multivitamins and 2 000 mg/kg multiminerals, the composition of them were shown in the reference[11]。

2)CP, Ca and TP were measured values, while the rest were calculated values.

1.2 检测指标与方法

1.2.1 生长性能

在试验第1天和第43天时以栏为单位称量各猪只的体重并记录耗料量,在称重前12 h对仔猪采取禁食措施。计算每组的平均日增重(ADG)、平均日采食量(ADFI),并根据ADG和ADFI计算料重比(F/G)。

1.2.2 肠道形态

试验第43天,从每栏随机挑选1头仔猪进行屠宰,环切约1 cm的十二指肠(近端)、空肠(中段)、回肠(远端),用注射器吸取磷酸盐缓冲液(PBS)轻轻冲洗后分别置于4%多聚甲醛样品瓶中固定保存,后续进行肠道形态学检测:经过冲水、脱水、透明、石蜡包埋等处理后,苏木精-伊红(HE)染色切片观察,每张切片测量9个完整的肠道绒毛及其伴生的隐窝,最后计算绒毛高度与隐窝深度的比值(V/C)。

1.2.3 肠黏膜基因表达

用实时荧光定量PCR的方法测定肠道屏障功能相关基因相对表达量,方法如下:利用Trizol Reagent(Invitrogen,美国)提取肠黏膜中的总RNA,接着反转录合成cDNA。后续PCR扩增反应体系为10 μL:Premix Taq 5 μL,上、下游引物各0.5 μL,cDNA模板2 μL,超纯水2 μL。试验所需引物均由Primer Premier 5.0软件设计,引物合成由上海生工生物工程有限公司完成,引物序列信息见表2。内参基因为β-肌动蛋白(β-actin),目的基因相对表达量用2-△△Ct法计算。
表2 引物序列信息

Table 2 Primer sequence information

基因
Genes
引物序列
Primer sequence (5'—3')
产物长度
Product size/bp
登录号
Accession number
闭锁小带蛋白-1
ZO-1
F: AGCCCGAGGCGTGTTT
R: GGTGGGAGGATGCTGTTG
147 XM_013993251
闭合蛋白
Occludin
F: GCACCCAGCAACGACAT
R: CATAGACAGAATCCGAATCAC
144 XM_005672525
黏液素-1
MUC-1
F: ACACCCATGGGCGCTATGT
R: GCCTGCAGAAACCTGCTCAT
68 NM-001204296.1
黏液素-2
MUC-2
F: CTGCTCCGGGTCCTGTGGGA
R: CCCGCTGGCTGGTGCGATAC
100 XM_007465997.1
猪beta防御素2
pBD2
F: CCAGAGGTCCGACCACTACA
R: GGTCCCTTCAATCCTGTTGAA
88 AY506573.1
猪beta防御素3
pBD3
F: CCTTCTCTTTGCCTTGCTCTT
R: GCCACTCACAGAACAGCTACC
163 NM_214444.1
抗菌肽1-5
PG1-5
F: GTAGGTTCTGCGTCTGTGTCG
R: CAAATCCTTCACCGTCTACCA
166 XM_005669497.2
Toll样受体2
TLR2
F: TCACTTGTCTAACTTATCATCCTCTTG
R: TCAGCGAAGGTGTCATTATTGC
162 NM_213761.1
Toll样受体4
TLR4
F: GCCATCGCTGCTAACATCATC
R: CTCATACTCAAAGATACACCATCGG
108 NM_001113039.1
β-肌动蛋白
β-actin
F: CTGCGGCATCCACGAAACT
R: AGGGCCGTGATCTCCTTCTG
380 XM_003124280

1.3 数据统计分析

数据采用SPSS 25.0统计软件进行单因素方差分析(one-way ANOVA),Duncan氏法进行多重比较。结果用平均值±均值标准误(mean±SEM)表示,GraphPad Prism软件作图,P<0.05表示差异显著。

2 结果与分析

2.1 猪源罗伊氏乳杆菌对断奶后42 d仔猪生长性能的影响

表3可知,LR1组相比于CON组平均日采食量有增加的趋势,但无显著差异(P>0.05),平均日增重显著提高了16.10%(P<0.05)。AO组平均日采食量较CON组显著增加了14.81%(P<0.05),平均日增重显著增加了19.22%(P<0.05)。与CON组相比,LR1组和AO组的腹泻率均有下降的趋势,但差异不显著(P>0.05)。
表3 猪源罗伊氏乳杆菌对断奶后42 d仔猪生长性能的影响

Table 3 Effects of Lactobacillus reuteri from pigs on growth performance of piglets at 42 days after weaning

项目
Items
组别 Groups P
P-value
CON AO LR1
初始体重 Initial body weight/kg 6.50±0.01 6.48±0.02 6.49±0.01 0.604
终末体重 Final body weight/kg 20.91±0.53b 23.29±0.64a 22.66±0.48a 0.017
平均日采食量 ADFI/(g/d) 605.42±16.89b 695.07±22.09a 658.04±26.30ab 0.024
平均日增重 ADG/(g/d) 331.72±13.16b 395.46±16.13a 385.12±13.90a 0.011
料重比 F/G 1.84±0.05 1.77±0.05 1.71±0.03 0.166
腹泻率 Diarrhea rate/% 11.66±2.81 7.84±2.49 8.11±1.98 0.481

同行数据肩标不同字母表示差异显著(P<0.05)。下表同。

In the same row, values with different letter superscripts mean significant difference (P<0.05). The same as below.

2.2 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道形态的影响

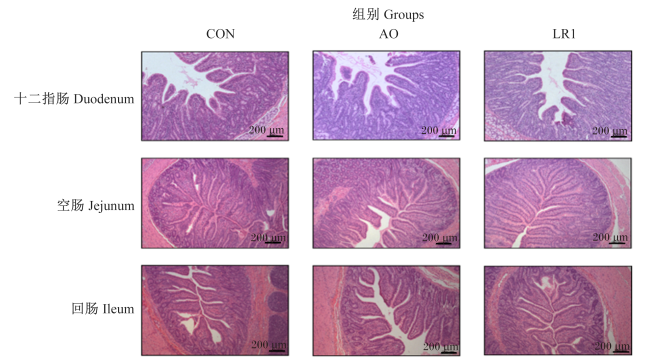
表4可知,与CON组和AO组相比,LR1组仔猪空肠和回肠的绒毛高度以及回肠的绒毛高度/隐窝深度显著提高(P<0.05)。此外,相比于CON组,LR1组十二指肠的绒毛高度与绒毛高度/隐窝深度也显著上升(P<0.05)。十二指肠、空肠及回肠的HE染色切片如图1所示,所有试验组猪小肠黏膜结构与形态完整。
表4 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道形态的影响

Table 4 Effects of Lactobacillus reuteri from pigs on intestinal morphology of piglets at 42 days after weaning

项目
Items
组别 Groups P
P-value
CON AO LR1
十二指肠 Duodenum
绒毛高度 Villus height/μm 371.08±17.80b 467.59±38.03a 485.18±19.17a 0.011
隐窝深度 Crypt depth/μm 381.45±24.99 383.53±25.61 325.47±47.50 0.410
绒毛高度/隐窝深度 V/C 1.02±0.09b 1.26±0.10ab 1.78±0.29a 0.022
空肠 Jejunum
绒毛高度 Villus height/μm 450.54±25.95b 433.06±21.23b 530.75±32.06a 0.045
隐窝深度 Crypt depth/μm 219.19±15.29 212.29±19.80 210.81±10.19 0.919
绒毛高度/隐窝深度 V/C 2.24±0.18 2.16±0.21 2.58±0.19 0.301
回肠 Ileum
绒毛高度 Villus height/μm 389.16±19.85b 376.34±25.24b 466.72±25.79a 0.034
隐窝深度 Crypt depth/μm 201.03±21.34 199.26±16.22 162.85±5.56 0.105
绒毛高度/隐窝深度 V/C 2.09±0.27b 1.98±0.11b 2.94±0.15a 0.001
图1 断奶仔猪肠道HE染色切片图

Fig.1 HE staining section map of intestinal tract of weaned piglets

2.3 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道上皮屏障功能的影响

2.3.1 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道紧密连接蛋白基因表达的影响
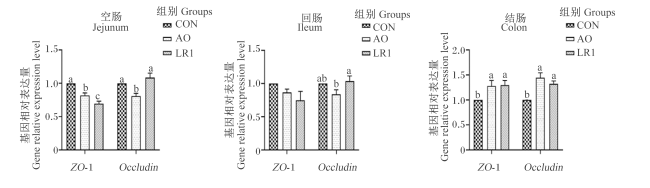
图2所示,LR1组与CON组相比,空肠闭锁小带蛋白-1(ZO-1)的基因相对表达量显著降低(P<0.05),结肠ZO-1与闭合蛋白(Occludin)的基因相对表达量显著增加(P<0.05)。与AO组相比,LR1组空肠以及回肠Occludin的基因相对表达量显著增加(P<0.05)。
图2 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道紧密连接蛋白基因表达的影响

ZO-1:闭锁小带蛋白-1 zonula occludens protein-1;Occludin:闭合蛋白。

CON:对照组;AO:抗生素组;LR1:罗伊氏乳杆菌组。柱状图上标不同字母表示差异显著(P<0.05)。下图同。

Fig.2 Effects of Lactobacillus reuteri from pigs on intestinal tight junction protein gene expression of piglets at 42 days after weaning

CON: control group; AO: antibiotic group; LR1: Lactobacillus reuteri group. Different letters of bar chart superscript mean significant difference (P<0.05). The same as below.

2.3.2 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道黏液素基因表达的影响

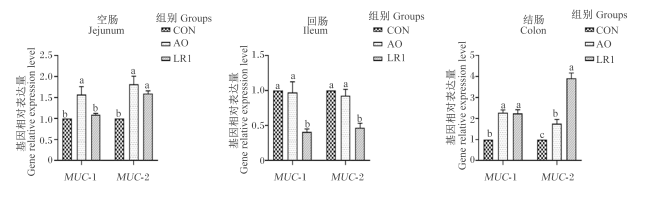
图3所示,LR1组的空肠黏液素-2(MUC-2)和结肠黏液素-1(MUC-1)、MUC-2的基因相对表达量显著高于CON组(P<0.05),回肠MUC-1、MUC-2基因相对表达量显著低于CON组(P<0.05)。与AO组相比,LR1组空肠MUC-1以及回肠MUC-1、MUC-2的基因相对表达量显著降低(P<0.05),显著增加了结肠MUC-2的基因相对表达量(P<0.05)。
图3 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道黏液素基因表达的影响

MUC-1:黏液素-1 mucin-1;MUC-2:黏液素-2 mucin-2。

Fig.3 Effects of Lactobacillus reuteri from pigs on intestinal mucin gene expression of piglets at 42 days after weaning

2.3.3 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道抗菌肽基因表达的影响

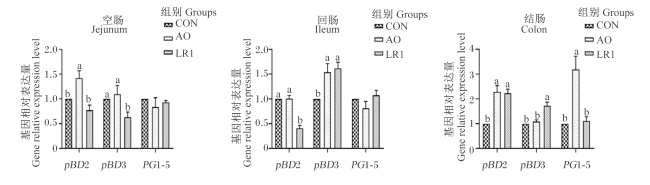
图4所示,与CON组相比,LR1组显著降低了空肠猪β防御素3(pBD3)、回肠猪β防御素2(pBD2)的基因相对表达量(P<0.05),显著增加了回肠pBD3、结肠pBD2、pBD3的基因相对表达量(P<0.05)。相较于AO组,LR1组显著降低了空肠pBD2、pBD3,回肠pBD2以及结肠抗菌肽1-5(PG1-5)的基因相对表达量(P<0.05),显著增加了结肠pBD3的基因相对表达量(P<0.05)。
图4 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道抗菌肽基因表达的影响

pBD2:猪beta防御素2 porcine beta defensin 2;pBD3:猪beta防御素3 porcine beta defensin 3;PG1-5:抗菌肽1-5 antimicrobial peptides 1-5。

Fig.4 Effects of Lactobacillus reuteri from pigs on intestinal antimicrobial peptide gene expression of piglets at 42 days after weaning

2.3.4 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道TLRs基因表达的影响

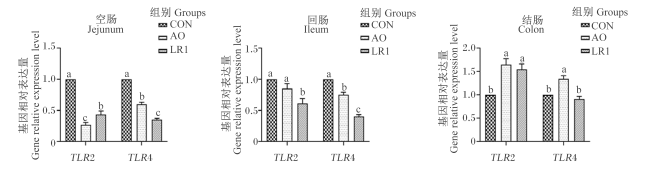
图5所示,LR1组的空肠和回肠Toll样受体2(TLR2)、Toll样受体4(TLR4)的基因相对表达量显著低于CON组(P<0.05),但与CON组相比显著增加了结肠TLR2的基因相对表达量(P<0.05)。与AO组相比,LR1组显著增加了空肠TLR2的基因相对表达量(P<0.05),显著降低了空肠、回肠以及结肠TLR4的基因相对表达量(P<0.05),同时显著降低了回肠TLR2的基因相对表达量(P<0.05)。
图5 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道TLRs基因表达的影响

TLR2:Toll样受体2 Toll-like receptors 2;TLR4:Toll样受体4 Toll-like receptors 4。

Fig.5 Effects of Lactobacillus reuteri from pigs on intestinal TLRs gene expression of piglets at 42 days after weaning

3 讨论

3.1 猪源罗伊氏乳杆菌对断奶后42 d仔猪生长性能的影响

抗生素是抗菌剂,可用于杀死肠道中的致病微生物,减轻免疫系统的负担,优化消化系统,改善生长性能[12]。本试验中,抗生素提高了仔猪的平均日增重以及平均日采食量。然而,在动物生产中持续使用抗生素导致了一系列抗生素耐药性病原体,这些病原体也影响人类和动物。因此,养殖中控制抗生素的用量尤为重要。我国已于2020年7月1日起“全面禁抗”,为了克服由于该禁令而导致的断奶仔猪死亡率、发病率和断奶后腹泻率增加的问题,已经提出了许多替代方案。益生菌是一种活的微生物,当给予足够的量时,通过不同的机制能够赋予宿主良好的健康效果,此前已被多项试验证实能够促进动物的生长发育[13-15]。LR是益生菌中较常见的一种,能够预防一些疾病或者改善疾病症状。本试验研究结果表明,LR1显著提高了仔猪断奶后42 d的末重和平均日增重,对平均日采食量也有提高的趋势。之前在鸡的研究上,已经证实LR有助于增加体重并降低饲料转化率[16],并有研究报道,饲粮中添加LR增加了仔猪断奶后42 d的末重和平均日增重[17]。本研究结果与以上研究结果一致。此外,本课题组前期研究发现,LR1可显著增加断奶后14 d的生长性能[8],说明LR1在断奶前期或断奶后42 d均能提高断奶仔猪的生长性能,在促生长型抗生素替代品中有良好的发展潜力。

3.2 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道形态的影响

小肠表面具有手指状微尺度的绒毛结构,它能扩大肠道表面积以利于宿主有效吸收,同时,其与隐窝结构对于肠上皮的结构完整性和维持肠道稳态也至关重要[18-19]。隐窝-绒毛组织结构与快速细胞更新相结合,使肠道既是营养吸收的主要部位,也是防止有害物质和病原体入侵的第1道屏障[20]。有研究表明,仔猪饲喂鼠李糖乳杆菌后,肠道绒毛高度显著挺高,且绒毛高度/隐窝深度也显著增加[21]。Moturi等[22]从猪的粪便中分离的唾液乳杆菌对仔猪肠道的绒毛高度也有显著促进作用。本研究结果表明,饲粮中添加LR1的仔猪其十二指肠、空肠以及回肠的绒毛高度均有显著的增加,并能改善十二指肠以及回肠的绒毛高度/隐窝深度。这与上述研究结果一致,表明LR1可通过提高仔猪的绒毛高度以及绒毛高度/隐窝深度来促进营养物质的吸收。

3.3 猪源罗伊氏乳杆菌对断奶后42 d仔猪肠道上皮屏障功能的影响

肠道屏障的稳态在很大程度上取决于TJ,当TJ发生改变时,可导致肠道屏障功能的快速恶化,最终阻碍正常的吸收和分泌活动[23]。TJ由位于肠上皮细胞侧膜顶端部分的多蛋白复合物形成,主要由跨膜蛋白(Occludin、Claudins)和支架蛋白(ZO-1和ZO-2)组成,在维持肠道物理屏障和调节肠道通透性方面起重要作用[24]。抗生素会破坏肠道正常微生物平衡,引起肠道屏障功能障碍[25]。本试验结果表明,饲用抗生素显著降低了仔猪空肠的ZO-1以及Occludin的基因表达,这和上述研究结果一致。但抗生素却增加了结肠ZO-1以及Occludin的基因表达,我们推测是由于结肠内容物较空肠、回肠来说停留时间较长、肠道菌群较为丰富的原因所造成的差异。LR1也表现出和抗生素一样的结果,降低了空肠ZO-1的基因表达,增加了结肠ZO-1以及Occludin的基因表达。但较抗生素来说,饲喂LR1增加了空肠、回肠Occludin的基因表达。先前研究表明,LR可以增加卵清蛋白致敏的大鼠空肠ZO-1、OccludinClaudin-1的基因表达[26]。本课题组在前期研究中也发现,LR1可显著增加断奶后仔猪早期小肠的ZO-1以及Occludin的表达[8],表明LR1能增强断奶早期仔猪的肠上皮物理屏障功能。但本试验中,LR1降低了空肠ZO-1的表达,说明LR1在断奶早期的效果比断奶中期好。此外,有研究发现LR FN041可以预防高脂肪饮食诱导的肠道屏障损伤,增加小鼠结肠OccludinZO-1的基因表达[27],这和本试验LR1增加仔猪结肠TJ的基因表达的结果一致,表明LR1能通过增加结肠ZO-1以及Occludin的基因表达来增强结肠的物理屏障功能。
紧密的上皮形成物理屏障,由黏液层进一步保护,黏液层提供各种特定部位的保护功能[28]。黏液素是胃肠道黏膜屏障的守门人,在各种胃肠道病理中异常表达[29],其主要成分为MUC-1和MUC-2,在肠道上皮黏液层中起着至关重要的作用。肠道黏液层厚度在空肠、回肠、结肠中依次增加。本试验中,LR1增加了空肠、结肠MUC-1、MUC-2的基因表达,却降低了回肠MUC-1、MUC-2的基因表达。此前研究报道,小鼠口服植物乳杆菌PS128增加了结肠MUC-2的量[30],LR能显著增加结肠黏液层的厚度[4],减少了肠腔细菌与肠上皮细胞的接触而不触发炎症反应,这和本试验中LR1增加结肠MUC-1、MUC-2的基因表达结果一致,说明LR1可通过增加黏液素的表达加强结肠的肠道屏障功能。
维持肠道稳态不仅需要耐受共生微生物群,还需要遏制入侵的病原体。越来越多的证据表明,潘氏细胞分泌的抗菌肽在先天肠道免疫和肠道微生物群调节中起着至关重要的作用[31]。研究发现,LR I5007对仔猪空肠以及回肠的抗菌肽调控作用不大,但能显著增加结肠中抗菌肽的表达,如pBD2、pBD3、pBD114等[32]。本试验结果表明,LR1显著降低了空肠pBD3、回肠pBD2的基因表达,但显著增加了回肠pBD3、结肠pBD2、pBD3的基因表达。结肠中微生物消化的主要代谢产物为短链脂肪酸,且短链脂肪酸可以诱导猪宿主抗菌肽基因表达[33]。有研究证实,饲喂发酵乳杆菌后可以显著增加结肠消化物中丁酸盐的含量[34],因此我们猜测造成空肠、回肠、结肠这种表达差异的原因可能是丁酸介导的。
Toll样受体是微生物诱导的蛋白质,在大多数上皮细胞谱系中表达,具有重要的抗菌功能,可动态调节肠上皮在宿主和肠道微生物群之间的物理和免疫屏障[35]。TLR2和TLR4是肠道稳态的关键介质。前人研究表明,新生仔猪饲喂鼠李糖乳杆菌后,空肠黏膜TLR2、TLR9基因表达水平显著上调[36],乳酸杆菌能显著上调新生仔猪回肠中TLR2、TLR4、TLR6和TLR9等的mRNA丰度,并显著上调了结肠TLR4的mRNA丰度。本试验研究结果表明,LR1组的空肠以及回肠的TLR2、TLR4的基因表达显著降低,但显著上调了结肠的TLR2的基因表达。这和前人研究结果部分保持一致,但与乳杆菌能提高空肠以及回肠中Toll样受体的表达相反。在新生仔猪中,肠黏膜屏障的完整性存在缺陷,早期饲喂LR1对断奶过渡期间微生物群发育以及猪健康影响显著。由于断奶后42 d时仔猪相比于刚断奶的仔猪来说具有更为完善的胃肠道功能,且体内的消化酶活性、免疫功能以及抗病能力增强,因此乳酸菌对断奶后42 d猪的影响相对有限[37]。大肠中的微生物组与小肠中的微生物组不同,并且比小肠中的微生物组更稳定[38],这可能是结肠不论是在前期或者后期都保持结果稳定的原因。

4 结论

饲粮中添加5×10¹⁰ CFU/kg猪源LR1可提高仔猪断奶后1~42 d的平均日增重,改善小肠绒毛高度与绒毛高度/隐窝深度,显著增加仔猪结肠紧密连接蛋白、黏液素、抗菌肽及Toll样受体基因的表达。由此可见,猪源LR1能够改善断奶后42 d仔猪生长性能、小肠绒毛形态及结肠肠道上皮屏障功能。
[1]
吴胜男, 胡胜兰, 蒋宗勇, 等. 罗伊氏乳杆菌调节肠黏膜屏障功能的作用及机制[J]. 动物营养学报, 2021, 33(9):4861-4869.

DOI

WU S N, HU S L, JIANG Z Y, et al. Role and mechanism of Lactobacillus reuteri in regulating intestinal mucosal barrier function[J]. Chinese Journal of Animal Nutrition, 2021, 33(9):4861-4869. (in Chinese)

[2]
WANG T T, ZHENG N S, LUO Q, et al. Probiotics Lactobacillus reuteri abrogates immune checkpoint blockade-associated colitis by inhibiting group 3 innate lymphoid cells[J]. Frontiers in Immunology, 2019, 10:1235.

DOI

[3]
LIU Y Y, TIAN X J, HE B K, et al. Lactobacillus reuteri DSM 17938 feeding of healthy newborn mice regulates immune responses while modulating gut microbiota and boosting beneficial metabolites[J]. American Journal of Physiology:Gastrointestinal and Liver Physiology, 2019, 317(6):G824-G838.

DOI

[4]
AHL D, LIU H, SCHREIBER O, et al. Lactobacillus reuteri increases mucus thickness and ameliorates dextran sulphate sodium-induced colitis in mice[J]. Acta Physiologica, 2016, 217(4):300-310.

DOI

[5]
YANG F J, WANG A N, ZENG X F, et al. Lactobacillus reuteri I5007 modulates tight junction protein expression in IPEC-J2 cells with LPS stimulation and in newborn piglets under normal conditions[J]. BMC Microbiology, 2015, 15:32.

DOI

[6]
YI H B, WANG L, XIONG Y X, et al. Lactobacillus reuteri LR1 improved expression of genes of tight junction proteins via the MLCK pathway in IPEC-1 cells during infection with enterotoxigenic Escherichia coli K88[J]. Mediators of Inflammation, 2018, 2018:6434910.

[7]
WANG Z L, WANG L, CHEN Z, et al. In vitro evaluation of swine-derived Lactobacillus reuteri:probiotic properties and effects on intestinal porcine epithelial cells challenged with enterotoxigenic Escherichia coli K88[J]. Journal of Microbiology and Biotechnology, 2016, 26(6):1018-1025.

DOI

[8]
YI H B, WANG L, XIONG Y X, et al. Effects of Lactobacillus reuteri LR1 on the growth performance,intestinal morphology,and intestinal barrier function in weaned pigs[J]. Journal of Animal Science, 2018, 96(6):2342-2351.

DOI

[9]
GAO J C, CAO S T, XIAO H, et al. Lactobacillus reuteri 1 enhances intestinal epithelial barrier function and alleviates the inflammatory response induced by enterotoxigenic Escherichia coli K88 via suppressing the MLCK signaling pathway in IPEC-J2 cells[J]. Frontiers in Immunology, 2022, 13:897395.

DOI

[10]
YANG K M, JIANG Z Y, ZHENG C T, et al. Effect of Lactobacillus plantarum on diarrhea and intestinal barrier function of young piglets challenged with enterotoxigenic Escherichia coli K88[J]. Journal of Animal Science, 2014, 92(4):1496-1503.

DOI

[11]
杨广达, 王丽, 易宏波, 等. 罗伊氏乳杆菌LR1对断奶仔猪血清生化指标和肠道营养物质转运载体mRNA表达的影响[J]. 动物营养学报, 2018, 30(11):4589-4600.

YANG G D, WANG L, YI H B, et al. Effects of Lactobacillus reuteri LR1 on serum biochemical indexes and mRNA expressions of intestinal nutrient transporters of weaned piglets[J]. Chinese Journal of Animal Nutrition, 2018, 30(11):4589-4600. (in Chinese)

[12]
MEHDI Y, LÉTOURNEAU-MONTMINY M P, GAUCHER M L, et al. Use of antibiotics in broiler production:global impacts and alternatives[J]. Animal Nutrition, 2018, 4(2):170-178.

DOI

[13]
LU X H, ZHANG M, ZHAO L, et al. Growth performance and post-weaning diarrhea in piglets fed a diet supplemented with probiotic complexes[J]. Journal of Microbiology and Biotechnology, 2018, 28(11):1791-1799.

DOI PMID

[14]
ABDELQADER A, ABUAJAMIEH M, HAYAJNEH F, et al. Probiotic bacteria maintain normal growth mechanisms of heat stressed broiler chickens[J]. Journal of Thermal Biology, 2020, 92:102654.

DOI

[15]
LI Y Y, JIA D, WANG J H, et al. Probiotics isolated from animals in northwest China improve the intestinal performance of mice[J]. Frontiers in Veterinary Science, 2021, 8:750895.

DOI

[16]
BHOGOJU S, KHWATENGE C N, TAYLOR-BOWDEN T, et al. Effects of Lactobacillus reuteri and Streptomyces coelicolor on growth performance of broiler chickens[J]. Microorganisms, 2021, 9(6):1341.

DOI

[17]
TANG Q S, YI H B, HONG W B, et al. Comparative effects of L. plantarum CGMCC 1258 and L. reuteri LR1 on growth performance,antioxidant function,and intestinal immunity in weaned pigs[J]. Frontiers in Veterinary Science, 2021, 8:728849.

DOI

[18]
ALLAIRE J M, CROWLEY S M, LAW H T, et al. The intestinal epithelium:central coordinator of mucosal immunity[J]. Trends in Immunology, 2018, 39(9):677-696.

DOI

[19]
KIM W J, KIM G H. An intestinal model with a finger-like villus structure fabricated using a bioprinting process and collagen/SIS-based cell-laden bioink[J]. Theranostics, 2020, 10(6):2495-2508.

DOI PMID

[20]
GEHART H, CLEVERS H. Tales from the crypt:new insights into intestinal stem cells[J]. Nature Reviews Gastroenterology & Hepatology, 2019, 16(1):19-34.

[21]
WANG Q, SUN Q, QI R L, et al. Effects of Lactobacillus plantarum on the intestinal morphology,intestinal barrier function and microbiota composition of suckling piglets[J]. Journal of Animal Physiology and Animal Nutrition, 2019, 103(6):1908-1918.

DOI

[22]
MOTURI J, KIM K Y, HOSSEINDOUST A, et al. Effects of Lactobacillus salivarius isolated from feces of fast-growing pigs on intestinal microbiota and morphology of suckling piglets[J]. Scientific Reports, 2021, 11(1):6757.

DOI

[23]
ROSE E C, ODLE J, BLIKSLAGER A T, et al. Probiotics,prebiotics and epithelial tight junctions:a promising approach to modulate intestinal barrier function[J]. International Journal of Molecular Sciences, 2021, 22(13):6729.

DOI

[24]
HAGIHARA M, KUROKI Y, ARIYOSHI T D H, et al. Clostridium butyricum modulates the microbiome to protect intestinal barrier function in mice with antibiotic-induced dysbiosis[J]. iScience, 2020, 23(1):100772.

DOI

[25]
ZHU L Y, LI J, WEI C H, et al. A polysaccharide from Fagopyrum esculentum Moench bee pollen alleviates microbiota dysbiosis to improve intestinal barrier function in antibiotic-treated mice[J]. Food & Function, 2020, 11(12):10519-10533.

[26]
TULYEU J, KUMAGAI H, JIMBO E, et al. Probiotics prevents sensitization to oral antigen and subsequent increases in intestinal tight junction permeability in Juvenile-young adult rats[J]. Microorganisms, 2019, 7(10):463.

DOI

[27]
LI S Q, QI C, ZHU H L, et al. Lactobacillus reuteri improves gut barrier function and affects diurnal variation of the gut microbiota in mice fed a high-fat diet[J]. Food & Function, 2019, 10(8):4705-4715.

[28]
CORNICK S, TAWIAH A, CHADEE K. Roles and regulation of the mucus barrier in the gut[J]. Tissue Barriers, 2015, 3(1/2):e982426.

DOI

[29]
JOHANSSON M E V, HANSSON G C. Immunological aspects of intestinal mucus and mucins[J]. Nature Reviews Immunology, 2016, 16(10):639-649.

DOI PMID

[30]
CHEN C M, WU C C, HUANG C L, et al. Lactobacillus plantarum PS128 promotes intestinal motility,mucin production,and serotonin signaling in mice[J]. Probiotics and Antimicrobial Proteins, 2022, 14(3):535-545.

DOI

[31]
CHUNG L K, RAFFATELLU M.G.I. pros:antimicrobial defense in the gastrointestinal tract[J]. Seminars in Cell & Developmental Biology, 2019, 88:129-137.

[32]
LIU H B, HOU C L, WANG G, et al. Lactobacillus reuteri I5007 modulates intestinal host defense peptide expression in the model of IPEC-J2 cells and neonatal piglets[J]. Nutrients, 2017, 9(6):559.

DOI

[33]
ZENG X F, SUNKARA L T, JIANG W Y, et al. Induction of porcine host defense peptide gene expression by short-chain fatty acids and their analogs[J]. PLoS One, 2013, 8(8):e72922.

DOI

[34]
LIU H, ZHANG J, ZHANG S H, et al. Oral administration of Lactobacillus fermentum I5007 favors intestinal development and alters the intestinal microbiota in formula-fed piglets[J]. Journal of Agricultural and Food Chemistry, 2014, 62(4):860-866.

DOI

[35]
BURGUEÑO J F, ABREU M T. Epithelial Toll-like receptors and their role in gut homeostasis and disease[J]. Nature Reviews Gastroenterology & Hepatology, 2020, 17(5):263-278.

[36]
WANG Y, GONG L, WU Y P, et al. Oral administration of Lactobacillus rhamnosus GG to newborn piglets augments gut barrier function in pre-weaning piglets[J]. Journal of Zhejiang University-SCIENCE B, 2019, 20(2):180-192.

DOI

[37]
YANG F J, HOU C L, ZENG X F, et al. The use of lactic acid bacteria as a probiotic in swine diets[J]. Pathogens, 2015, 4(1):34-45.

DOI PMID

[38]
LIU Y, ZHENG Z J, YU L H, et al. Examination of the temporal and spatial dynamics of the gut microbiome in newborn piglets reveals distinct microbial communities in six intestinal segments[J]. Scientific Reports, 2019, 9(1):3453.

DOI PMID

Outlines

/