REVIEW

Research Progress on Agouti-Related Peptide/Pro-Opiomelanocortin Neurons in Regulation of Fish Feeding

  • JIN Xiaoyan ,
  • CHEN Xiumei , * ,
  • LIN Yunjie ,
  • WANG Guiqin
Expand
  • Key Laboratory for Animal Production, Product Quality and Safety of Ministry of Education, Jilin Provincial Key Laboratory of Animal Nutrition and Feed Science, College of Animal Science and Technology, Jilin Agriculture University, Changchun 130118, China
* lecturer, E-mail:

Received date: 2023-06-07

  Online published: 2023-12-11

Abstract

Feeding is crucial for fish survival, growth, development and reproduction. The feeding process is mainly regulated by the central nervous system of the hypothalamus, among which agouti-related peptide (AgRP) neurons and pro-opiomelanocortin (POMC) neurons are the two key neurons to control feeding. Through combing domestic and foreign literature, based on an overview of the neurons and distribution of AgRP/POMC, this paper analyzes the role of AgRP/POMC neurons in the regulation of feeding, and explores the strategy of regulating fish feeding based on the AgRP/POMC neuron pathway, in order to provide reference for the study of feeding regulation in fish and other aquatic animals.

Key words: AgRP; POMC; fish; feeding; regulation

Cite this article

JIN Xiaoyan , CHEN Xiumei , LIN Yunjie , WANG Guiqin . Research Progress on Agouti-Related Peptide/Pro-Opiomelanocortin Neurons in Regulation of Fish Feeding[J]. Chinese Journal of Animal Nutrition, 2023 , 35(12) : 7595 -7604 . DOI: 10.12418/CJAN2023.689

鱼类的生长与摄食密切相关,可通过摄食行为获得食物,用于维持个体的生存、生长、发育和生殖。下丘脑是机体调节摄食及能量代谢的中枢,同样也是内分泌系统的中枢,它能感知并整合各种信号分子调节摄食。下丘脑弓状核存在许多与能量调控相关的神经元,在调节摄食和能量代谢中起着至关重要的作用。鱼类的摄食机制十分复杂,涉及一系列信号调节因子,刺鼠相关蛋白(agouti-related peptide,AgRP)神经元与阿片黑素促皮质激素原(pro-opiomelanocortin,POMC)神经元的相互作用是其主要的调控机制之一。这2种神经元对摄食的调节功能截然相反,AgRP神经元增强饥饿感,POMC神经元则增强饱腹感,二者相互作用,形成一个开关系统,能即时快速地调整摄食行为。本文以AgRP/POMC神经元为切入点,系统了解AgRP/POMC神经元对鱼类摄食的调节机理,对今后水产养殖业的高效和绿色发展有着重要意义。目前,AgRP/POMC神经元在哺乳动物及畜禽中已经进行了深入研究,关于鱼类食欲的研究相对浅显且零散。因此,本文主要概述这2种关键神经元及其分布,分析其在摄食调节中的作用,并基于AgRP/POMC神经元途径探究调控鱼类摄食的策略,以期为鱼类等水产动物摄食调控的深入研究提供一定的参考依据。

1 AgRP/POMC神经元概述

1.1 AgRP神经元

AgRP最早于1997年在寻找刺鼠信号蛋白同源基因时被发现,由AgRP基因所编码,也被称之为大鼠相关肽,是一种有效且持久的摄食刺激因子,AgRP表达量增加时能提高食物的摄入量,被认为是强有力的能量平衡调节剂[1]。AgRP主要分布在下丘脑弓状核处,并与神经肽Y(neuropeptide Y,NPY)产生共表达,所以被命名为AgRP/NPY神经元,又名AgRP神经元[2]。随着对AgRP了解的深入,又因为发现其会同时分泌NPY、AgRP和γ-氨基丁酸(γ-aminobutyric acid,GABA),也被称为NAG神经元。它可通过激活胰岛素受体(insulin receptor,IR)和瘦素受体(leptin receptor,LepR)收取外周糖、脂代谢的大部分信号分子,进而增加食物摄入行为以获得稳态所需要的能量[3]。有研究表明,若通过化学遗传学技术去降低AgRP神经元的活性,能明显减小进食行为[4],且此神经元的基因消融会导致饥饿[5];相比之下,光遗传学或化学遗传学技术可以刺激AgRP神经元使食物摄取快速且可逆的增加[4,6]。因此,AgRP神经元被认为在调节摄食,尤其促进食欲过程中发挥重要作用。

1.2 POMC神经元

1979年,有学者发现牛促肾上腺皮质激素(adrenocorticotropic hormone,ACTH)和β-脂肪酸释放激素(β-lipotropic hormone,β-LPH)基因是由同一个基因所编码的前体蛋白剪切得到的,由于这种前体蛋白能够产生阿片类物质β-内啡肽、ACTH和α,β,γ-促黑素细胞激素(melanocyte stimulating hormone,MSH)等,被认为是抑制摄食和增加能量消耗的肽类物质[7],因此将其称为POMC,其所在的神经元被称为POMC神经元。禁食条件下POMCα-MSH转录本表达水平降低,摄食条件下其表达水平升高。在垂体中,前叶中促肾上腺素细胞中的POMC被加工为ACTH,促进肾上腺分泌加工皮质醇,参与到机体的应激反应,而缺乏ACTH会导致动物机体肾上腺功能受损。迄今为止,POMC基因及其类似的mRNA或核苷酸序列已经在哺乳动物[8]、鸟类[9-10]、爬行动物[11-12]、鱼类[13-14]等众多脊椎动物和无脊椎动物中被发现,而大部分真骨鱼类POMC只编码2个MSH序列[15]。以上大量研究结果表明,POMC作为动物大脑和垂体中各种活性肽和激素的常见前体,是代谢和繁殖的关键调节因子。

2 AgRP/POMC神经元组织分布

AgRP在中枢神经系统和外周组织上都有表达,主要高表达于下丘脑、丘脑核和肾上腺中,在睾丸、肺脏、肾脏、脊髓和背根神经节中有少量表达[16]。同样鱼类上也有类似的报道,有研究人员运用荧光定量PCR技术测定了齐口裂腹鱼(Schizothorax prenanti)各个组织和胚胎时期AgRP基因的表达分布,结果表明AgRP在各个组织中的表达量从高到低分别为:脑、精巢、卵巢、垂体、眼、心脏和肝胰腺,在胚胎期,未受精卵、受精卵和卵裂时AgRP mRNA的表达量较低[17]。同样在检测AgRP基因在金钱鱼(Scatophagus argus)的表达情况时发现,AgRP基因产生表达主要在下丘脑、肌肉和脑垂体处。
POMC基因在中枢神经系统和外周组织中组织表达,在垂体中有高表达量[18]POMC具有细胞特异性表达,在正常生理条件下,只有下丘脑和垂体POMC基因通过垂体特异性启动子编码有生物活性的POMC蛋白,垂体外组织才会分泌具有生物活性的POMC相关蛋白[19-20]。与哺乳动物类似,鱼类POMC也广泛存在于机体各处的组织器官,如斑点叉尾 (Ictalurus punctatus)的脑组织[21],南方鲇(Silurus meridionalis Chen)的间脑、中脑、嗅球,虹鳟(Oncorhynchus mykiss)的间脑、中脑、延髓和端脑,稀有 鲫(Gobiocypris rarus)的大脑均有一定的表达量。在刀鲚(Coilia nasus)上的研究发现,POMC基因在脑中高表达,其次较高表达于鳃、肾脏、精巢组织中,最后微表达于肝脏、脾脏、肠道、肾脏、肌肉和卵巢组织中[18]。综上研究报道,AgRP基因和POMC基因在中枢神经系统和外周组织广泛分布,提示二者可能在多种生理功能中发挥重要作用。

3 AgRP/POMC神经元在摄食调节中的作用
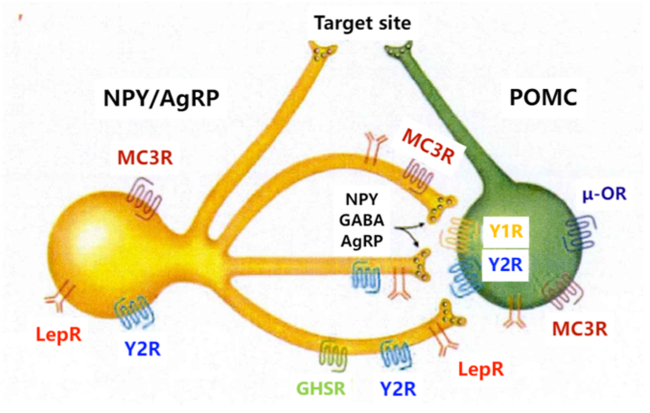
AgRP/POMC神经元对于摄食可以发挥调节作用,并且分别体现在促进与抑制2个方面(图1)。促进方面具体表现为AgRP神经元投射至POMC神经元胞体,并控制POMC神经元而促进进食[3]。目前这2种神经元尚未发现直接突触连接,2个神经元的相反作用部分是通过对同一信号机制施加相反作用的相同效应神经元介导的。AgRP是α-MSH的竞争性拮抗剂,能与黑素皮质素受体(melanocortin receptor,MCR)中的黑素皮质素3受体(melanocortin 3 receptor,MC3R)和黑素皮质素4受体(melanocortin 4 receptor,MC4R)竞争结合,α-MSH作为激素传递的信息需要通过体液的传送,然后与相应的靶细胞上的受体结合而发挥作用,AgRP作为神经元产生的神经递质传导兴奋在同一个神经元上是以电流的形式,只在突触处才转化为化学信号的形式,所以AgRP传导兴奋的速度快,能够抑制MSH通路激活,促进食物摄入[22]。哺乳动物体外和体内试验表明,AgRP也被认为是一种逆激动剂,可以独立于α-MSH的存在而调节MC3R和MC4R[23]。POMC是许多生物活性肽的前体蛋白,其产生的α-MSH和β-MSH作用于MC3R和MC4R以激活厌食反应[24]。而且POMC/AgRP神经元都表达LepRIR,并被各自的激素靶向,以此提高POMC的表达,并一定程度上缩减NPYAgRP的表达[25]。此外,2个神经元群体均可通过产生带有抑制作用的GABA,即神经递质来一定程度上抑制周围POMC神经元的激活能力[26-27]。综上所述,AgRP/POMC神经元互相作用形成一个完整的调控网络,共同调节摄食过程。
图1 下丘脑弓状核的AgRP/POMC神经元及相关信号分子

Target site:靶位点;NPY:神经肽Y neuropeptide Y;AgRP:刺鼠相关蛋白 agouti-related peptide;POMC:阿片黑素促皮质激素原 proopiomelanocortin;MC3R:黑素皮质素3受体 melanocortin 3 receptor;GABA:γ-氨基丁酸 γ-aminobutyric acid;Y1R:神经肽Y受体Y1 neuropeptide Y receptor Y1;Y2R:神经肽Y受体Y2 neuropeptide Y receptor Y2;μ-OR:μ型阿片受体 μ-opioid receptor;LepR:瘦素受体 leptin receptor;GHSR:生长激素促分泌素受体 recombinant growth hormone secretagogue receptor。

Fig.1 AgRP/POMC neurons and related signaling molecules in arcuate nucleus of hypothalamus[28]

3.1 AgRP神经元促进摄食

AgRP神经元能激发并促进摄食,主要通过2种方式识别和整合外部代谢信号。第一是神经途径,它是由副交感神经、迷走神经系统中的传递纤维组成,并通过AgRP神经元向下游的多个神经元群体进行投射[29]。第二是体液调节,这其中包含瘦素(Leptin)、胰岛素、胃饥饿素(Ghrelin)等化学物质及血液游离脂肪酸等各种类型的营养物质。
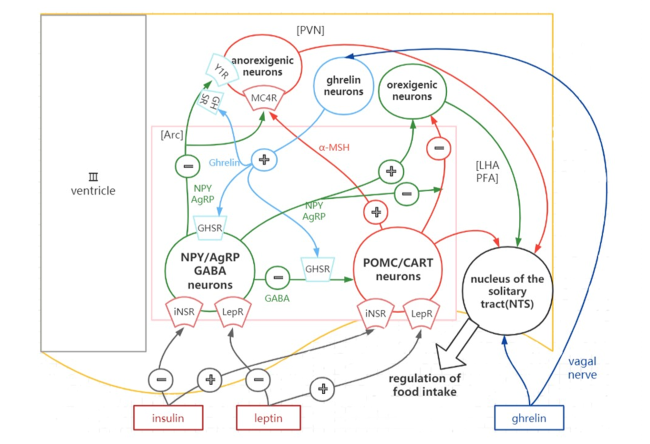
下丘脑室旁核作为一种神经元内扮演重要角色的内分泌和代谢调节团核,与第三脑室顶端相邻。前期研究发现,AgRP神经元能通过突触传递NPY和AgRP均向着室旁核释放,并很大程度上调控了摄食(图2,绿色线条部分)。POMC神经元也会把α-MSH分泌到室旁核神经元;α-MSH通过MC4R调控摄食;而AgRP能一定程度上抑制α-MSH,从而促进摄食[30]。当能量不足时,AgRP神经元所产生的AgRP蛋白肽会和α-MSH竞争与MC4R结合[31],拮抗α-MSH介导的鸟苷酸结合蛋白(G蛋白)活化,降低细胞内环腺苷酸含量,最后致使食欲提高。与此同时,在饥饿时下丘脑弓状核的NPY加速合成,再传给室旁核,在饱食中枢中发生作用,NPY受体Y1、Y2和Y3基因表达量显著增加,发挥促摄食作用,在金鱼(Carassius auratus)[32]、草鱼(Ctenopharyngodon idella)[33]、乌鳢(Channa argus)[34]中均证实了NPY基因很大程度上参与了摄食调控的过程。另外游离脂肪酸会被AgRP神经元吸收掉一部分,并通过这一过程被转化为“游离脂肪酸-辅酶A”,进而刺激神经元产生胞质脂滴,自噬相关基因7启动表达、自噬以及促进AgRP表达和借助NPY提高脂肪组织中的脂蛋白脂酶和己酰辅酶A羧化酶活性,刺激脂肪生成,从而提高摄食,减少基础代谢量,并增加脂肪储备[35]。刺激AgRP神经元可以抑制室旁丘脑核的食欲减退的神经元,间接恢复餐后岛叶皮层(insular cortex)的饥饿反应模式[36](图2,绿色线条部分)。AgRP神经元还可能向臂旁核发送γ-氨基丁酸能神经投射,直接或间接减少臂旁核中降钙素基因相关肽(calcitonin gene-related peptide,CGRP)神经元的影响程度。与这一假设相同的是,清除AgRP神经元,会提高CGRP神经元的活跃性[37-38],刺激AgRP向臂旁核神经投射,降低了CGRP神经元中艾塞那肽在臂旁核中的表达[38],进而刺激摄入食物的需求。
图2 摄食相关的神经内分泌调控途径

Ⅲ ventricle:第三脑室;PVN:室旁核 paraventricular nucleus;Arc:弓状核 arcuate nucleus;LHA:下丘脑外侧区 lateral hypothalamic area;PFA:穹隆周区 perifornical area;NTS:孤术核 nucleus of the solitary tract;vagel nerve:迷走神经;anorexigenic neurons:厌食肽神经元;ghrelin neurons:胃饥饿素神经元;orexigenic neurons:食欲肽神经元;Y1R:神经肽Y受体Y1 neuropeptide Y receptor Y1;MC4R:黑素皮质素4受体 melanocortin 4 receptor;GHSR:生长激素促分泌素受体 recombinant growth hormone secretagogue receptor;ghrelin:胃饥饿素;α-MSH:α-促黑素细胞激素 α-melanocyte stimulating hormone;NPY:神经肽Y neuropeptide Y;AgRP:刺鼠相关蛋白 agouti-related peptide;GABA:γ-氨基丁酸γ-aminobutyric acid;iNSR:胰岛素受体 insulin receptor;LepR:瘦素受体 leptin receptor;insulin:胰岛素;leptin:瘦素;regulation of food intake:摄食调控;POMC:阿片黑素促皮质激素原 pro-opiomelanocortin;CART:可卡因-苯丙胺调节转录因子 cocaine-and amphetamine-regulated transcript。

Fig.2 Neuroendocrine regulatory pathways related to food intake

有学者通过研究发现,爱帕琳肽(Apelin)可以用来激活5'-磷酸腺苷激活蛋白激酶(AMP-activated protein kinase,AMPK)路径,可以提高肌细胞对葡萄糖的摄取,还可以提高下丘脑NPY/AgRP和食欲素的表达水平,从而提高摄食效率。还可通过刺激磷脂酰肌醇3-激酶/蛋白激酶B(phosphatidylinositol 3-kinase/protein kinase B,PI3K/Akt)信号途径,提高脂肪组织摄取葡萄糖[39-42]。AgRP刺激食欲的效应也可通过抑制Leptin和激活Ghrelin来实现。Leptin对AgRP具有抑制作用,脂肪细胞在动物进食后会分泌瘦素,而Leptin能直接控制于AgRP/NPY神经元[43](图2,黑色线条部分)。叉头蛋白O1(forkhead box O1,FoxO1)是Leptin信号通路的负调控因子。在营养缺乏时,FoxO1由胞质移至胞核,上调NPY/AgRP基因表达水平,同时抑制POMC基因的表达水平,借此来提高了对食物的摄取需求[44]。雷帕霉素能使哺乳动物雷帕霉素靶蛋白(mammalian target of rapamycin,mTOR)活性下降,降低下游效应分子活性,增加AgRPGhrelin表达量,促进齐口裂腹鱼摄食[45]。当Ghrelin受到体活化时可以启动生长激素(growth hormone,GH)/AMPK信号途径,借此刺激神经元抑制性神经递质GABA的产生,进而减弱POMC神经元的放电频率,并抑制α-MSH的分泌[3],从而提高食物摄入,新陈代谢率降低,脂肪储存增加,体重增加(图2,黑蓝色线条部分)[46]

3.2 POMC神经元抑制食欲

POMC神经元对于维持能量稳态至关重要。POMC神经元的活化可调控摄食和降低摄食,其抑制摄食主要通过激活中枢MC4R来实现。POMC神经元产生POMC蛋白,是很多功能性蛋白肽的前体,如α-MSH、内啡肽(endorphins)和ACTH等[47]。其中,α-MSH是MC4R重要的激活配体,而MC4R则在体重调节中起着核心作用,激活MC4R可降低食欲,同时提高能量利用率[48]
有报道表明,金鱼在长期禁食条件下,其摄食能力显著增强,POMC的裂解可能更倾向于产生β-内啡肽,而在食物充足的情况下,POMC则优先产生摄食抑制剂α-MSH[49]。当机体脂肪含量增加时,由于Leptin受到刺激,在脂肪组织中的合成分泌开始增加,Leptin受体借助与酪氨酸激酶2的结合来实现与酪氨酸激酶2的磷酸化,并与受体蛋白的不同位置结合,从而激活相应的信号转导系统,导致AgRPNPY mRNA表达量下降,同时刺激下丘脑增强神经细胞POMC基因的表达;随着POMC基因的高度表达,其降解产物中α-MSH的含量逐渐提高,α-MSH开始与其进行受体结合,逐渐形成能够抑制食物摄取的生理效应(图2,红色线条部分)[50-51]。瘦素还可以借助PI3K途径启动PI3K磷酸化活化磷酸肌醇激酶1,进一步磷酸化活化Akt,再抑制下游的FoxO1,提高POMC的表达量,最后达到抑制摄食的作用[51]。此外,应用下丘脑移植技术,Goazigo等[52]研究发现,Apelin可促进POMC细胞内α-MSH的自分泌释放。还有研究中发现,Apelin能通过丝裂原激活蛋白激酶(mitogen-activated protein kinase,MAPK)途径,促进胆囊收缩素(cholecystokinin,CCK)的分泌,进而参与摄食调控[53-54]。在食物充足时,饱食因子α-MSH的释放量会借助Apelin-17显著提高,Apelin-13的分泌会被减少,而且食欲素和NPY的表达也会在一定程度上被抑制,并降低肠道内分泌细胞及近侧小肠细胞中胆囊收缩素的释放,与POMC共同抑制食欲,减少摄食量。氨基酸通常可以被用于调节环腺苷酸应答元件结合蛋白转录共激活因子CREB调节转录辅激活因子1(TORC1),但在大多数情况下更多的是起到抑制TORC1信号通路的作用进而降低食欲[55],在鱼类研究中发现,亮氨酸能够刺激mTOR,使其在下丘脑弓状核活化,由细胞内外的因素作用于细胞表面的受体或目标蛋白质,然后将信号传递给mTOR,又或者直接对其下游效应物的核糖体蛋白S6激酶1产生效果,减少Ghrelin分泌,同时增加POMC的表达量,降低齐口裂腹鱼摄食量[45]

4 基于AgRP/POMC神经元调控鱼类摄食的策略

目前,国内外的研究者已开展多种鱼类AgRP/POMC神经元生物学特性研究。尽管大多数研究都仅限于基因克隆,但与其他脊椎动物一样,鱼类的食物摄入调节涉及大脑和外周组织产生的大量激素,根据最新人、鼠及其他陆生动物的研究进展亦可为鱼类摄食调控提供思路。
在鱼类研究中发现,用100 ng食欲素或Apelin-13进行腹腔注射0.5 h后,洞穴鱼(Astyanax fasciatus mexicanus)AgRP基因的表达量明显升高,并且其摄食量明显提高,还能够消除POMC对食欲的抑制作用,从而促进摄食[56]。使用NPY(0.6 μg/g)10 h后,罗非鱼(Oreochromis mossambicus)AgRP基因的表达量明显提高,且其摄食能力明显增强[57],与此类似,注射Apelin(100 ng/g)、食欲素(100 ng/g)和Ghrelin(100 ng/g)会使斑马鱼(Astyanax fasciatus mexicanus)摄食量增加[58]。除此之外,在对金鱼的研究中,在腹腔注射Ghrelin(1~2 pmol/g)后,在45~60 min内可以明显提高其摄食量[59],在侧脑室(10 ng/g)和腹腔(100 ng/g)注射Apelin-13 1 h后,摄食量都显著提高[60]。在齐口裂腹鱼体内注入Apelin-13(100 ng/g)后,0.5 h时摄食量明显提高[61]。Apelin也可通过下调POMC的表达提高鲤摄取食物的需求[62]。结果表明,对研究对象注入合适剂量的食欲素、NPY、Ghrelin及Apelin,可以通过促进AgRP的表达又或者抑制POMC基因表达借助这2个途径提高鱼类的摄食能力。此外,在虹鳟脑室内注射Leptin可引起厌食肽POMCCART基因表达,降低其摄食量[63]。在金鱼体内注射试验中也证明了CCK对摄食的抑制作用[64-65]。因此,可以通过添加它们对应的拮抗剂解除POMC对食欲的抑制作用,从而促进摄食。一般而言,短期禁食会对食欲素、胃饥饿素等基因的表达有促进作用,对饱食因子(CARTCCK等)基因的表达有抑制作用。
但是,在不同的物种或禁食的持续时间不同,这种个体情况的差异都会使得个别食欲调节因子基因的表达量产生差异[66]。例如,在禁食72 h后金鱼脑内NPY基因的表达量明显增加,而在青鲈(Tautogolabrus adspersus)的禁食试验中却出现了与之相反的现象[67-68]。因此,对于一部分鱼类在鱼体健康环境适宜的情况下,可以采取短期禁食的方法促进食欲,提高摄食量。饲料中添加适宜的添加剂可以显著提升特定鱼类的饲料利用率,刺激生物的摄食需求,借此谋求更好的经济收益[69]。研究表明,α-脂肪酸(1 200 μg/kg)可通过抑制肠道食欲相关基因的表达,进而减少草鱼的摄食量[70]。石斑鱼(Epinephelus coioides)的摄食量增加可以通过在饲料中加入一定量的NPY(1 000、2 000 ng/g)实现[71],而对于增加罗非鱼的摄食可以选择在饵料中加入250 ng/g的NPY来实现[56]。研究发现,若要增加肠道Ghrelin mRNA的表达,可以选择在饲料中加入酸枣叶粉,且酸枣叶粉可以提高罗非鱼的摄食能力[72]。通过在饲料中添加功能适口性增强剂,可提高鱼体肝胰腺中蛋白酶的活性,从而更好地增加了采食量[73]。因此,可以通过在饲料中添加不同促食因子或功能性添加剂,以促进鱼类的摄食。Liang等[74]在草鱼的研究中发现,以植物蛋白质混合物为蛋白质源的饲料比以鱼粉作为蛋白质源的饲料有更好的饲料效应,GhrelinAgRP基因的表达上调的同时,LeptinPOMCPYY基因的表达下调,由此推断,外周和中枢食欲因子的差异性调节参与了鱼粉组食欲下降和植物蛋白质混合组主动觅食的状态;而在花鲈的研究中表明,饲料中鱼粉完全被植物蛋白质所替代时,鱼类厌食症导致的能量负平衡引起了胃中Ghrelin基因的表达上调和Leptin基因的表达下调,同时伴随着血浆中较高的Ghrelin浓度,表明外周器官对营养物质摄入不足的感知是有效的[75]。然而,下丘脑mTOR的激活降低了下游核糖体蛋白S6激酶1(S6K1)的磷酸化,同时伴随着厌食阶段厌食基因POMC表达的进一步上调和促食基因AgRP表达的下调[75]。因此,植物蛋白质引起的自发性厌食与摄食适应的调控机制需要进一步研究,这对改善鱼类的摄食、解决其带来了负面影响极为重要。

5 小结与展望

在模式动物上关于AgRP/POMC神经元结构、组织表达分布及其在摄食调控中的作用已经有了较为清晰的认知,但在鱼类上的研究尚零散,处于相关调控因子基因克隆及表达水平高低分析的层面,其作用机制及相关摄食调节因子功能并未深入探索。目前的研究结果已经提示AgRP/POMC神经元在鱼类摄食调控中的重要性,今后的研究工作主要集中于明确这2个神经元的中枢调节机制,理清其介导的各种摄食调节因子的作用途径及其交叉作用,并借助先进的分子生物学手段理顺鱼类机体特有的摄食调控信号通路,刻画鱼类摄食调控网络,这也是目前鱼类摄食调控研究的重点及难点,进而为通过营养途径调控鱼类摄食提供新思路,达到高效绿色健康养殖的目的。
[1]
VIVOT K, MESZAROS G, PANGOU E, et al. CaMK1D signalling in AgRP neurons promotes ghrelin-mediated food intake[J]. Nature Metabolism, 2023, 5(6):1045-1058.

DOI PMID

[2]
VOHRA M S, BENCHOULA K, SERPELL C J, et al. AgRP/NPY and POMC neurons in the arcuate nucleus and their potential role in treatment of obesity[J]. European Journal of Pharmacology, 2022, 915:174611.

DOI

[3]
王梦远, 王俊博, 唐致恒, 等. AgRP/NPY神经元代谢调控功能研究进展[J]. 生理科学进展, 2019, 50(1):67-75.

WANG M Y, WANG J B, TANG Z H, et al. Metabolic regulatory function of AgRP/NPY neurons[J]. Progress in Physiological Sciences, 2019, 50(1):67-75. (in Chinese)

[4]
FENG B, LIU H S, MISHRA I, et al. Asprosin promotes feeding through SK channel-dependent activation of AgRP neurons[J]. Science Advances, 2023, 9(8):eabq6718.

DOI

[5]
LUQUET S, PEREZ F A, HNASKO T S, et al. NPY/AgRP neurons are essential for feeding in adult mice but can be ablated in neonates[J]. Science, 2005, 310(5748):683-685.

DOI PMID

[6]
APONTE Y, ATASOY D, STERNSON S M. AGRP neurons are sufficient to orchestrate feeding behavior rapidly and without training[J]. Nature Neuroscience, 2011, 14(3):351-355.

DOI PMID

[7]
徐龙鑫, 朱丽莉, 张麟, 等. 关岭黄牛POMC基因多态性及其与生长性状的关联性分析[J]. 西南农业学报, 2016, 29(2):451-454.

XU L X, ZHU L L, ZHANG L, et al. Polymorphism of POMC gene in Guanling cattle and its association with growth traits[J]. Southwest China Journal of Agricultural Sciences, 2016, 29(2):451-454. (in Chinese)

[8]
ALJUBOURI T R S, AL-SHUHAIB M B S. A missense SNP in the proopiomelanocortin (POMC) gene is associated with growth traits in Awassi and Karakul sheep[J/OL]. Animal Biotechnology:1-14[2023-05-01].https://doi.org/10.1080/10495398.2023.2197469.

[9]
LIU K, WEN Y Y, LIU H H, et al. POMC gene expression,polymorphism,and the association with reproduction traits in chickens[J]. Poultry Science, 2020, 99(6):2895-2901.

DOI

[10]
RANCOURT R C, SCHELLONG K, TZSCHENTKE B, et al. DNA methylation and expression of proopiomelanocortin (POMC) gene in the hypothalamus of three-week-old chickens show sex-specific differences[J]. FEBS Open Bio, 2018, 8(6):932-939.

DOI

[11]
SHEN S T, LU L M, CHEN J R, et al. Molecular cloning of proopiomelanocortin (POMC) cDNA from mud turtle,Pelodiscus sinensis[J]. General and Comparative Endocrinology, 2003, 131(2):192-201.

DOI

[12]
SHOURESHI P, BARON A, SZYNSKIE L, et al. Analyzing the evolution of β-endorphin post-translational processing events:studies on reptiles[J]. General and Comparative Endocrinology, 2007, 153(1/2/3):148-154.

DOI

[13]
KALANANTHAN T, MURASHITA K, RØNNESTAD I, et al. Hypothalamic AgRP and POMC mRNA responses to gastrointestinal fullness and fasting in Atlantic salmon (Salmo salar,L.)[J]. Frontiers in Physiology, 2020, 11:61.

DOI

[14]
WAN Z Y, LIN V C L, HUA Y G. Pomc plays an important role in sexual size dimorphism in tilapia[J]. Marine Biotechnology, 2021, 23(2):201-214.

DOI PMID

[15]
丁炜东, 曹哲明, 曹丽萍. 鲇POMC cDNA的克隆与表达分析[J]. 中国水产科学, 2011, 18(5):1000-1010.

DING W D, CAO Z M, CAO L P. Molecular cloning of propiomelanocortin cDNA and multi-tissue mRNA expression in Parasilurus asotus[J]. Journal of Fishery Sciences of China, 2011, 18(5):1000-1010. (in Chinese)

DOI

[16]
BELTRAMO M, CAMPANELLA M, TAROZZO G, et al. Gene expression profiling of melanocortin system in neuropathic rats supports a role in nociception[J]. Molecular Brain Research, 2003, 118(1/2):111-118.

DOI

[17]
WEI R B, YUAN D Y, WANG T, et al. Characterization,tissue distribution and regulation of agouti-related protein (AgRP) in a cyprinid fish (Schizothorax prenanti)[J]. Gene, 2013, 527(1):193-200.

DOI

[18]
杜富宽, 徐钢春, 黎燕, 等. 刀鲚POMC基因的cDNA克隆及其应激应答[J]. 中国水产科学, 2017, 24(2):231-238.

DU F K, XU G C, LI Y, et al. Cloning of POMC cDNA and the stress response in Coilia nasus[J]. Journal of Fishery Sciences of China, 2017, 24(2):231-238. (in Chinese)

DOI

[19]
连小兰, 白耀. 脑类固醇的合成及其临床意义[J]. 国外医学(内分泌学分册), 2003, 23(5):334-337.

LIAN X L, BAI Y. Synthesis of cerebral steroids and its clinical significance[J]. Foreign Medical Sciences (Section of Endocrinology), 2003, 23(5):334-337. (in Chinese)

[20]
叶蕾, 宁光. POMC在异源ACTH综合征中的基因表达调控研究[J]. 国外医学(内分泌学分册), 2003, 23(5):337-340.

YE L, NING G. Study on gene expression regulation of POMC in allogenic ACTH syndrome[J]. Foreign Medical Sciences (Section of Endocrinology), 2003, 23(5):337-340. (in Chinese)

[21]
KARSI A, WALDBIESER G C, SMALL B C, et al. Molecular cloning of proopiomelanocortin cDNA and multi-tissue mRNA expression in channel catfish[J]. General and Comparative Endocrinology, 2004, 137(3):312-321.

PMID

[22]
LIMA L B, PEDROSO J A B, METZGER M, et al. Relationship of α-MSH and AgRP axons to the perikarya of melanocortin-4 receptor neurons[J]. Brain Research, 2019, 1717:136-146.

DOI PMID

[23]
TOLLE V, LOW M J. In vivo evidence for inverse agonism of agouti-related peptide in the central nervous system of proopiomelanocortin-deficient mice[J]. Diabetes, 2008, 57(1):86-94.

DOI

[24]
BIEBERMANN H, CASTAÑEDA T R, VAN LANDEGHEM F, et al. A role for β-melanocyte-stimulating hormone in human body-weight regulation[J]. Cell Metabolism, 2006, 3(2):141-146.

DOI

[25]
KITAMURA T, FENG Y, KITAMURA Y I, et al. Forkhead protein FoxO1 mediates AgRP-dependent effects of leptin on food intake[J]. Nature Medicine, 2006, 12(5):534-540.

PMID

[26]
SMITH M A, CHOUDHURY A I, GLEGOLA J A, et al. Extrahypothalamic GABAergic nociceptin-expressing neurons regulate AgRP neuron activity to control feeding behavior[J]. Journal of Clinical Investigation, 2020, 130(1):126-142.

DOI PMID

[27]
RAU A R, HENTGES S T. GABAergic inputs to POMC neurons originating from the dorsomedial hypothalamus are regulated by energy state[J]. Journal of Neuroscience, 2019, 39(33):6449-6459.

DOI PMID

[28]
MERCER R E, MICHAELSON S D, CHEE M J S, et al. Magel2 is required for leptin-mediated depolarization of POMC neurons in the hypothalamic arcuate nucleus in mice[J]. PLoS Genetics, 2013, 9(1):e1003207.

DOI

[29]
BETLEY J N, CAO Z F H, RITOLA K D, et al. Parallel,redundant circuit organization for homeostatic control of feeding behavior[J]. Cell, 2013, 155(6):1337-1350.

DOI

[30]
WATERSON M J, HORVATH T L. Neuronal regulation of energy homeostasis:beyond the hypothalamus and feeding[J]. Cell Metabolism, 2015, 22(6):962-970.

DOI

[31]
HE X F, LU Z, MA B B, et al. Chronic heat stress alters hypothalamus integrity,the serum indexes and attenuates expressions of hypothalamic appetite genes in broilers[J]. Journal of Thermal Biology, 2019, 81:110-117.

DOI

[32]
LI J X, CHEN T, RAOY Z, et al. Suppression of leptin-AⅠ/AⅡ transcripts by insulin in goldfish liver:a fish specific response of leptin under food deprivation[J]. General and Comparative Endocrinology, 2019, 283:113240.

DOI

[33]
方龙, 梁旭方, 何珊. 草鱼禁食后NPY与血糖变化及NPY重组表达[J]. 暨南大学学报(自然科学与医学版), 2013, 34(5):533-538.

FANG L, LIANG X F, HE S. The variation of NPY and blood glucose after fasting and recombinant expression of NPY in grass carp[J]. Journal of Jinan University (Natural Science & Medicine Edition), 2013, 34(5):533-538. (in Chinese)

[34]
文正勇, 覃川杰, 邹远超, 等. 乌鳢神经肽Y基因的克隆、组织表达及功能研究[C]// 2017年中国水产学会学术年会论文摘要集. 南昌: 中国水产学会, 2017:349.

WEN Z Y, QIN C J, ZOU Y C, et al. Molecular cloning,tissue expression and functional identification of neuropeptide Y gene in Channa argus[C]// Abstractions of Papers of the 2017 Annual Conference of Chinese Society of Fisheries. Nanchang: China Society of Fisheries, 2017:349. (in Chinese)

[35]
KAUSHIK S, RODRIGUEZ-NAVARRO J A, ARIAS E, et al. Autophagy in hypothalamic AgRP neurons regulates food intake and energy balance[J]. Cell Metabolism, 2011, 14(2):173-183.

DOI PMID

[36]
LIVNEH Y, RAMESH R N, BURGESS C R, et al. Homeostatic circuits selectively gate food cue responses in insular cortex[J]. Nature, 2017, 546(7660):611-616.

DOI

[37]
WU Q, BOYLE M P, PALMITER R D. Loss of GABAergic signaling by AgRP neurons to the parabrachial nucleus leads to starvation[J]. Cell, 2009, 137(7):1225-1234.

DOI PMID

[38]
CAMPOS C A, BOWEN A J, SCHWARTZ M W, et al. Parabrachial CGRP neurons control meal termination[J]. Cell Metabolism, 2016, 23(5):811-820.

DOI PMID

[39]
SAVOVA M S, MIHAYLOVA L V, TEWS D, et al. Targeting PI3K/AKT signaling pathway in obesity[J]. Biomedicine & Pharmacotherapy, 2023, 159:114244.

DOI

[40]
YUE P, JIN H, AILLAUD M, et al. Apelin is necessary for the maintenance of insulin sensitivity[J]. American Journal of Physiology:Endocrinology and Metabolism, 2010, 298(1):E59-E67.

DOI

[41]
ATTANÉ C, DAVIAUD D, DRAY C, et al. Apelin stimulates glucose uptake but not lipolysis in human adipose tissue ex vivo[J]. Journal of Molecular Endocrinology, 2011, 46(1):21-28.

DOI

[42]
ZHU S M, SUN F, LI W J, et al. Apelin stimulates glucose uptake through the PI3K/Akt pathway and improves insulin resistance in 3T3-L1 adipocytes[J]. Molecular and Cellular Biochemistry, 2011, 353(1/2):305-313.

DOI

[43]
BAVER S B, HOPE K, GUYOT S, et al. Leptin modulates the intrinsic excitability of AgRP/NPY neurons in the arcuate nucleus of the hypothalamus[J]. Journal of Neuroscience, 2014, 34(16):5486-5496.

DOI PMID

[44]
TEANEY N A, CYR N E. Sirtuin 1 regulates synapsin 1 in POMC-producing N43-5 neurons via FOXO1[J]. Journal of the Endocrine Society, 2021,5 (Suppl.1):A56-A57.

[45]
LIN F J, CHEN H, LIU J, et al. Molecular cloning of a proglucagon in a cyprinid fish (Schizothorax prenanti):mRNA tissue distribution and quantification during periprandial changes and fasting[J]. Aquaculture, 2015, 448:250-255.

DOI

[46]
MOUNTJOY K G. Pro-opiomelanocortin (POMC) neurones,POMC-derived peptides,melanocortin receptors and obesity:how understanding of this system has changed over the last decade[J]. Journal of Neuroendocrinology, 2015, 27(6):406-418.

DOI

[47]
TAO M, JI R L, HUANG L, et al. Regulation of melanocortin-4 receptor pharmacology by two isoforms of melanocortin receptor accessory protein 2 in topmouth culter (Culter alburnus)[J]. Frontiers in Endocrinology, 2020, 11:538.

DOI

[48]
马天瀛, 李怡霖, 董心玥, 等. 食物摄入与下丘脑能量平衡[J]. 畜牧兽医学报, 2021, 52(7):1789-1799.

MA T Y, LI Y L, DONG X Y, et al. Food intake and hypothalamic energy balance[J]. Acta Veterinaria et Zootechnica Sinica, 2021, 52(7):1789-1799. (in Chinese)

[49]
PILOZZI A, CARRO C, HUANG X D. Roles of β-endorphin in stress,behavior,neuroinflammation,and brain energy metabolism[J]. International Journal of Molecular Sciences, 2020, 22(1):338.

DOI

[50]
FERRAO R D, WALLWEBER H J, LUPARDUS P J. Receptor-mediated dimerization of JAK2 FERM domains is required for JAK2 activation[J]. eLife, 2018, 7:e38089.

DOI

[51]
DERGHAL A, ASTIER J, SICARD F, et al. Leptin modulates the expression of miRNAs-targeting POMC mRNA by the JAK2-STAT3 and PI3K-Akt pathways[J]. Journal of Clinical Medicine, 2019, 8(12):2213.

DOI

[52]
GOAZIGO A, BODINEAU L, DE MOTA N D, et al. Apelin and the proopiomelanocortin system:a new regulatory pathway of hypothalamic α-MSH release[J]. American Journal of Physiology-Endocrinology and Metabolism, 2011, 301(5):E955-E966.

DOI

[53]
WANG G Y, ANINI Y, WEI W, et al. Apelin,a new enteric peptide:localization in the gastrointestinal tract,ontogeny,and stimulation of gastric cell proliferation and of cholecystokinin secretion[J]. Endocrinology, 2004, 145(3):1342-1348.

DOI

[54]
CAMPOS C A, WRIGHT J S, CZAJA K, et al. CCK-induced reduction of food intake and hindbrain MAPK signaling are mediated by NMDA receptor activation[J]. Endocrinology, 2012, 153(6):2633-2646.

DOI PMID

[55]
SAUCISSE N, MAZIER W, SIMON V, et al. Functional heterogeneity of POMC neurons relies on mTORC1 signaling[J]. Cell Reports, 2021, 37(2):109800.

DOI

[56]
PENNEY C C, VOLKOFF H. Peripheral injections of cholecystokinin,apelin,ghrelin and orexin in cavefish (Astyanax fasciatus mexicanus):effects on feeding and on the brain expression levels of tyrosine hydroxylase,mechanistic target of rapamycin and appetite-related hormones[J]. General and Comparative Endocrinology, 2014, 196:34-40.

DOI

[57]
KIRIS G A, KUMLU M, DIKEL S. Stimulatory effects of neuropeptide Y on food intake and growth of Oreochromis niloticus[J]. Aquaculture, 2007, 264(1/2/3/4):383-389.

DOI

[58]
BÜLBÜL M, SINEN O, BIRSEN Ī, et al. Peripheral apelin-13 administration inhibits gastrointestinal motor functions in rats:the role of cholecystokinin through CCK1 receptor-mediated pathway[J]. Neuropeptides, 2017, 63:91-97.

DOI

[59]
MATSUDA K, MIURA T, KAIYA H, et al. Stimulatory effect of n-octanoylated ghrelin on locomotor activity in the goldfish,Carassius auratus[J]. Peptides, 2006, 27(6):1335-1340.

DOI

[60]
VOLKOFF H, WYATT J L. Apelin in goldfish (Carassius auratus):cloning,distribution and role in appetite regulation[J]. Peptides, 2009, 30(8):1434-1440.

DOI

[61]
LIN F J, WU H W, CHEN H, et al. Molecular and physiological evidences for the role in appetite regulation of apelin and its receptor APJ in Ya-fish (Schizothorax prenanti)[J]. Molecular and Cellular Endocrinology, 2014, 396(1/2):46-57.

DOI

[62]
YAN X, QIN C B, DENG D P, et al. Apelin and apj in common carp (Cyprinus carpio L.):molecular characterization,tissue expression and responses to periprandial changes and fasting-refeeding[J]. Aquaculture Research, 2020, 51(3):1012-1025.

DOI

[63]
GONG N P, JÖNSSON E, BJÖRNSSON B T. Acute anorexigenic action of leptin in rainbow trout is mediated by the hypothalamic PI3K pathway[J]. Journal of Molecular Endocrinology, 2016, 56(3):227-238.

DOI PMID

[64]
WALL A, VOLKOFF H. Effects of fasting and feeding on the brain mRNA expressions of orexin,tyrosine hydroxylase (TH),PYY and CCK in the Mexican blind cavefish (Astyanax fasciatus mexicanus)[J]. General and Comparative Endocrinology, 2013, 183:44-52.

DOI

[65]
SACHURIGA, IINUMA N, SHIBATA H, et al. Intracerebroventricular administration of sulphated cholecystokinin octapeptide induces anxiety-like behaviour in goldfish[J]. Journal of Neuroendocrinology, 2019, 31(1):e12667.

DOI

[66]
BERTUCCI J I, BLANCO A M, SUNDARRAJAN L, et al. Nutrient regulation of endocrine factors influencing feeding and growth in fish[J]. Frontiers in Endocrinology, 2019, 10:83.

DOI PMID

[67]
MIKWAR M, NAVARRO-MARTIN L, XING L, et al. Stimulatory effect of the secretogranin-ll derived peptide secretoneurin on food intake and locomotion in female goldfish (Carassius auratus)[J]. Peptides, 2016, 78:42-50.

DOI PMID

[68]
BABICHUK N A, VOLKOFF H. Changes in expression of appetite-regulating hormones in the cunner (Tautogolabrus adspersus) during short-term fasting and winter torpor[J]. Physiology & Behavior, 2013, 120:54-63.

DOI

[69]
邓茂刚. 绿色饲料添加剂综述[J]. 山东畜牧兽医, 2007, 29(2):36-38.

DENG M G. Review of green feed additives[J]. Shandong Journal of Animal Science and Veterinary Medicine, 2007, 29(2):36-38. (in Chinese)

[70]
HUANG C C, SUN J, JI H, et al. Influence of dietary alpha-lipoic acid and lipid level on the growth performance,food intake and gene expression of peripheral appetite regulating factors in juvenile grass carp (Ctenopharyngodon idellus)[J]. Aquaculture, 2019, 505:412-422.

DOI

[71]
WU S G, LI B, LIN H R, et al. Stimulatory effects of neuropeptide Y on the growth of orange-spotted grouper (Epinephelus coioides)[J]. General and Comparative Endocrinology, 2012, 179(2):159-166.

DOI PMID

[72]
AMIN A, EL ASELY A, ABD EL-NABY A S, et al. Growth performance,intestinal histomorphology and growth-related gene expression in response to dietary Ziziphus mauritiana in Nile tilapia (Oreochromis niloticus)[J]. Aquaculture, 2019, 512:734301.

DOI

[73]
ZHU T T, MORAIS S, LUO J X, et al. Functional palatability enhancer improved growth,intestinal morphology,and hepatopancreas protease activity,replacing squid paste in white shrimp,Litopenaeus vannamei,diets[J]. Journal of the World Aquaculture Society, 2019, 50(6):1064-1077.

DOI

[74]
LIANG X F, YU X T, HAN J, et al. Effects of dietary protein sources on growth performance and feed intake regulation of grass carp (Ctenopharyngodon idellus)[J]. Aquaculture, 2019, 510:216-224.

DOI

[75]
LIANG X F, HAN J, XUE M, et al. Growth and feed intake regulation responses to anorexia,adaptation and fasting in Japanese seabss,Lateolabrax japonicas when fishmeal is totally replaced by plant protein[J]. Aquaculture, 2019, 498:528-538.

DOI

Outlines

/