RESEARCH PAPER

Effects of Replacing Soybean Meal with Milk Thistle Meal on Growth Performance, Blood Biochemical Indexes, Liver Antioxidant Indexes and Metabolism Related Gene Expression of Lambs

  • ZHAO Meng , 1 ,
  • REN Yanbo 2 ,
  • DU Ruiping 1 ,
  • SONG Liwen 1 ,
  • HE Zhixiong 3 ,
  • GAO Min , 1
Expand
  • 1 Institute of Animal Nutrition and Feed Science, Inner Mongolia Academy of Agricultural & Animal Husbandry Sciences, Hohhot 010031, China
  • 2 College of Animal Science, Inner Mongolia Agricultural University, Hohhot 010018, China
  • 3 Institute of Subtropical Agriculture, Chinese Academy of Sciences, Changsha 410125, China
**professor, E-mail:

*Contributed equally

Received date: 2023-10-15

  Online published: 2024-04-15

Abstract

The main purpose of this experiment was to investigate the effects of replacing soybean meal with milk thistle meal on the growth performance, blood biochemical indexes, liver antioxidant indexes and metabolism related gene expression of lambs. Sixty-three Hulunbuir lambs with similar body weight and good physical condition were selected as experimental animals and were randomly divided into 3 groups with 7 replicates of 3 sheep per replicate. The proportions of replacing soybean meal with milk thistle meal in the three diets were 0 (group Ⅰ), 50% (group Ⅱ) and 100% (group Ⅲ), respectively. The experimental period was a total of 90 days, with a pre feeding period of 27 days and a trial period of 63 days. Weighed and recorded the experimental lambs every month during the experimental period, and recorded the feed intake every day. After the experiment, nine lambs were randomly selected from each group for blood collection, and three lambs were slaughtered to collect liver tissue samples for subsequent testing. The results showed as follows: 1) the growth performance of lambs in groups Ⅰ, Ⅱ and Ⅲ had no significant difference (P>0.05). 2) There were no significant differences in serum metabolic indexes among groups Ⅰ, Ⅱ and Ⅲ (P>0.05); the plasma interleukin-1β (IL-1β), tumor necrosis factor-α (TNF-α), transforming growth factor-β (TGF-β), hepatocyte growth factor (HGF), vascular endothelial cell growth factor (VEGF) contents of lambs in group Ⅲ were significantly higher than those in group Ⅰ (P≤0.05), but the insulin-like growth factor-1 (IGF-1) and interleukin-2 (IL-2) contents were not significantly different among groups (P>0.05). 3) There were no significant differences in liver antioxidant indexes among groups (P>0.05). Among them, the antioxidant capacity (T-AOC), the activities of glutathione peroxidase (GSH-Px) and superoxide dismutase (SOD) in liver in group Ⅲ were higher than those in group Ⅰ (P>0.05), and the malondialdehyde (MDA) content in group Ⅲ was lower than that in group Ⅰ (P>0.05). 4) The relative expression levels of liver lipid metabolism related genes acetyl-CoA acyltransferase 1 (ACAA1), aldehyde dehydrogenase 3 family member A2 (ALDH3A2) and fatty acid synthase (FASN) in group Ⅲ were higher than those in group Ⅰ, but the differences were not significant (P>0.05); the relative expression level of liver glucose metabolism related gene fructose-bisphosphatase 1 (FBP1) in group Ⅲ was significantly higher than that in group Ⅰ (P≤0.05), and the relative expression levels of phosphoenolpyruvate carboxykinase 2 (PCK2) and glucose-6-phosphatase catalytic subunit (G6PC) were higher than those in group Ⅰ, but the differences were not significant (P>0.05); the relative expression levels of liver tricarboxylic acid cycle pathway related genes succinate dehydrogenase complex subunit B (SDHB)and succinate dehydrogenase complex subunit C (SDHC) in group Ⅲ were significantly higher than those in group Ⅰ (P<0.05), and the relative expression level of isocitrate dehydrogenase 3β subunit (IDH3B) was higher than those in group Ⅰ, but the difference was not significant (P>0.05). Therefore, using milk thistle meal to replace soybean meal in the diet does not have a negative impact on growth performance and liver metabolism of lambs. Simultaneously, it can enhance the contents of immune cytokines in blood, and helps improving disease resistance. Moreover, the milk thistle meal can improve liver antioxidant capacity, upregulate liver metabolic gene expression, and accelerate energy metabolism cycle of lambs, so the milk thistle meal has a positive effect on production.

Cite this article

ZHAO Meng , REN Yanbo , DU Ruiping , SONG Liwen , HE Zhixiong , GAO Min . Effects of Replacing Soybean Meal with Milk Thistle Meal on Growth Performance, Blood Biochemical Indexes, Liver Antioxidant Indexes and Metabolism Related Gene Expression of Lambs[J]. Chinese Journal of Animal Nutrition, 2024 , 36(4) : 2524 -2540 . DOI: 10.12418/CJAN2024.217

豆粕为我国传统养殖业的主要饲料原料,因其含有丰富的蛋白质和满足动物机体所需的氨基酸组成,是理想的蛋白质饲料。随着畜牧业的高速发展,我国对豆粕的需求不断攀升,豆粕价格也水涨船高。近年来,随着国际竞争的加剧,豆粕不足已经成为制约我国畜牧业健康稳定发展的重要因素。为保障我国畜牧业健康稳定地可持续发展,豆粕减量替代研究势在必行,国内相关从业企业以及科研院所专家越来越重视非常规饲料资源的应用研究和新型蛋白质饲料的开发,新型蛋白质饲料资源的开发应用可以从根源上解决我国养殖业对豆粕的依赖,从而促进国内畜牧业健康稳定发展。水飞蓟,属于菊科水飞蓟属,有很强的环境气候适应性,是一种高1.2 m左右的一至两年生草本植物。水飞蓟最早被德国药学家用来治疗肝炎相关疾病,其药用成分被命名为水飞蓟素或西利马灵(silymarin)[1]。据报道,水飞蓟素对于多种肝胆类疾病有着不错的预防和治疗效果,还能够增强机体的免疫力和抗氧化能力等[2-5]。因此,水飞蓟大多被用来提取水飞蓟素以药物形式利用[6]。另有研究表明,水飞蓟不仅含有一定的药用价值,而且还有很高的营养价值,其蛋白质含量丰富,氨基酸种类可满足动物所需,是一种理想的具有药用价值的豆粕替代性新型蛋白质饲料[7]
我国于20世纪70年代从德国引进水飞蓟进行种植推广,主要种植地区为辽宁、黑龙江等地,作为药用植物,其产区主要围绕药物生产呈现区域性聚集种植。由于其仅用于药物生产这单一渠道,受产销因素波动,其种植面积及产量也呈现大幅波动,市场佳时种植面积高达百万亩,产量达10万t,市场低迷时种植面积骤减九成,产量也仅为1万t左右[8]。水飞蓟籽加工提取水飞蓟素后剩余的水飞蓟残渣为水飞蓟粕,优质的水飞蓟粕中含有25%~30%的粗蛋白质,具有成为植物性蛋白质饲料的潜质[9]。但对水飞蓟粕作为新型蛋白质饲料的开发与应用目前还处于初级阶段,水飞蓟粕没有得到合理的开发利用,造成了资源的浪费[10-11]。张松柏[12]研究了饲粮中不同比例水飞蓟粕替代豆粕对肉牛生长性能、屠宰指标及牛肉品质的影响,结果表明水飞蓟粕替代豆粕可在不影响生长性能的前提下降低饲料成本,增加生产利润。孙婷婷等[13]的研究显示,在保证基础饲粮中其他营养成分不改变的情况下,以水飞蓟粕代替25%、50%、75%豆粕,通过与对照组(基础饲粮)相比,水飞蓟粕可以提高獭兔的平均日增重、平均日采食量以及皮张面积,其中以水飞蓟粕代替50%豆粕时得到的效果最佳。吴峰洋等[14]的研究表明,水飞蓟粕可以作为家兔生长过程中的蛋白质饲料进行应用。Vojtísek等[15]通过对产后代谢病高发阶段的奶牛进行水飞蓟粕添加饲喂试验发现,饲粮中添加0.3 kg/(头·d)剂量的水飞蓟粕可以显著降低患代谢病奶牛血液和牛奶中的丙酮和β-羟丁酸含量,且使产奶量提高了7.7%,从而证明水飞蓟粕对奶牛酮病有一定的治疗效果。Li等[16]的研究表明,利用水飞蓟残渣固态发酵后对饲料的品质进行改良具有一定的潜在价值。Hashemi等[17]通过在不同代谢能水平的饲粮中添加不同水平的水飞蓟粕来研究其对蛋鸡生产性能、血液生化指标、肠道组织学的影响,结果表明水飞蓟粕添加在蛋鸡饲粮中具有较好的抗氧化性和抗菌性,可以改善蛋鸡的健康指标和生产性能。综上所述,水飞蓟粕作为饲料原料已经开始研究并应用到畜禽生产中,但水飞蓟粕在反刍动物饲粮中作为替代豆粕的新型蛋白质饲料的添加比例以及对反刍动物生产性能的影响等问题目前还有待进一步研究。因此,本试验将水飞蓟粕替代饲粮中不同比例的豆粕,研究其对羔羊生长性能、生理机能及肝脏代谢的影响,以期进一步完善水飞蓟粕作为反刍动物新型蛋白质饲料原料的应用价值以及水飞蓟粕替代豆粕用于反刍动物饲粮的可行性,同时为促进我国肉羊产业安全、绿色、可持续发展以及对豆粕替代性新型饲料资源开发利用提供可参考资料。

1 材料与方法

1.1 试验设计

选取63只体重相近、体况良好、3月龄左右的呼伦贝尔断奶羔羊,随机分为3组,每组设7个重复,每个重复3只羊。3组饲粮中水飞蓟粕替代豆粕的比例依次为0(Ⅰ组)、50%(Ⅱ组)和100%(Ⅲ组)。水飞蓟粕的主要营养成分含量见表1。试验饲粮营养水平参照《肉羊营养需要量》(NY/T816—2021)设计,其组成及营养水平见表2。试验全期90 d,包括27 d的预试期和63 d的正试期。
表1 试验饲粮组成及营养水平(风干基础)

Table 1 Composition and nutrient levels of experimental diets (air-dry basis)%

项目 Items Ⅰ组 Group Ⅰ Ⅱ组 Group Ⅱ Ⅲ组 Group Ⅲ
原料 Ingredients
小麦秸秆 Wheat straw 5.00 5.00 5.00
苜蓿 Alfalfa 30.00 30.00 30.00
玉米 Corn 30.50 30.50 30.50
大麦Barley 5.60 5.60 5.60
小麦麸 Wheat bran 11.00 11.00 11.00
豆粕 Soybean meal 10.00 5.00 0.00
水飞蓟粕 Milk thistle meal 5.00 10.00
棉籽粕 Cottonseed meal 3.00 3.00 3.00
小苏打 NaHCO3 0.70 0.70 0.70
食盐 NaCl 0.50 0.50 0.50
碳酸钙 CaCO3 0.50 0.50 0.50
氧化镁 MgO 0.20 0.20 0.20
甜菜糖蜜 Beet molasses 1.00 1.00 1.00
预混料 Premix1) 2.00 2.00 2.00
合计 Total 100.00 100.00 100.00
营养水平 Nutrient levels2)
代谢能 ME/(MJ/kg) 10.46 10.29 10.11
干物质 DM 90.82 89.88 90.06
粗蛋白质 CP 14.82 13.11 12.83
酸性洗涤纤维 ADF 6.81 6.71 6.66
中性洗涤纤维 NDF 23.93 22.83 22.66
钙 Ca 0.86 0.84 0.82
总磷 TP 0.31 0.33 0.35

1)预混料为每千克饲粮提供 The premix provided the following per kilogram of diets: Fe 221.31 mg,Cu 16.23 mg,Zn 71.31 mg,Mn 71.31 mg,I 1.23 mg,Co 0.54 mg,Se 1.70 mg,VA 16 250 IU,VD 5 000 IU,VE 40 IU。

2)干物质、粗蛋白质、中性洗涤纤维、酸性洗涤纤维、钙、总磷均为实测值,代谢能为计算值[18]。DM, CP, NDF, ADF, Ca and TP were measured values, while ME was a calculated value[18].

表2 水飞蓟粕的主要营养成分含量(风干基础)

Table 2 Main nutritional component contents of milk thistle meal (air-dry basis)[14]

项目
Item
总能
GE/
(MJ/kg)
干物质
DM/%
粗灰分
Ash/%
粗蛋白质
CP/%
粗纤维
CF/%
中性洗
涤纤维
NDF/%
酸性洗
涤纤维
ADF/%
粗脂肪
EE/%

Ca/%

P/%
水飞蓟粕
Milk thistle meal
17.12 91.94 5.31 23.62 16.21 38.57 22.73 2.07 0.29 0.68

1.2 饲养管理

在预试期对羊群进行编号、驱虫、称重,并且按照羔羊育肥的正常免疫程序对其进行预防免疫。在整个试验期间保证羊舍光照充足、通风,每3 d清理1次羊粪以保证羊舍的清洁卫生;每周对羊舍进行1次消毒处理;3组试验羊分3群管理,每天凌晨以群为单位按照各自组别饲粮组成采用小型全混合日粮(TMR)搅拌机进行拌料饲喂。各组试验羊均单栏自由采食,保证每次投料时料槽中有5%~10%的剩料量,每天饲喂及添水3次,分别于06:00、11:00和18:00进行饲喂和添水,并保证水槽和料槽洁净。

1.3 样品及数据采集

1.3.1 饲粮样本采集

于每日饲喂时采集100 g饲粮样本装入密封袋于4 ℃冰箱内保存,试验结束后冷藏运输回实验室4 ℃冰箱保存,用于营养成分测定。

1.3.2 体重数据采集

分别于试验第1天、第30天、第60天和第90天测定羔羊体重,测定选取凌晨喂料前羔羊空腹状态进行。

1.3.3 血液样本采集及血清、血浆分离

在试验结束当天,每组随机选取9只羊于晨饲前采用颈静脉穿刺方式采血,并分别使用10 mL乙二胺四乙酸二钾(EDTA-K2)抗凝采血管及非抗凝采血管收集,之后将非抗凝采血管斜置于4 ℃冰箱中静置30 min,待血液凝固后3 000 r/min离心15 min,收集血清移至1.5 mL离心管内-20 ℃保存,用于后续血清代谢指标分析;将抗凝采血管于采样2 h内4 ℃保存移至实验室,之后3 000 r/min离心10 min,收集血浆于1.5 mL冻存管中-20 ℃保存,用于血浆细胞因子含量测定。

1.3.4 肝脏组织样本采集及组织匀浆上清液制备

在试验结束当天,每组随机选择3只羔羊进行屠宰,屠宰后取肝脏组织,用无菌生理盐水冲洗后,剪碎至1 cm大小组织块放入冻存管液氮冻存,移至实验室-80 ℃冰箱保存备用。
将肝脏样品从超低温冰箱中取出,放入研钵中加液氮研磨至粉末状;称取2 g肝脏组织粉末于2.5 mL EP管内,随后加入1.8 mL的生理盐水,振荡匀浆;将制备好的肝脏组织匀浆置于1.5 mL离心管中,3 000 r/min离心15 min,离心后取上清液于1.5 mL EP管内,分装多管后置于-80 ℃冰箱保存备用。

1.4 指标检测与方法

1.4.1 营养成分

饲粮中水分、粗蛋白质、中性洗涤纤维、酸性洗涤纤维、钙、总磷分别参照GB/T 6435—2014、GB/T 6432—2018、GB/T 20806—2022、NY/T 1459—2022、GB/T 6436—2018、GB/T 6437—2018测定。

1.4.2 生长性能

记录每天饲粮的投喂量和剩余量,记录试验羔羊体重数据。根据以下公式计算生长性能指标:
平均日采食量(average daily feed intake,ADFI)=总采食量/试验天数;
平均日增重(average daily gain,ADG)=总增重/试验天数;
料重比(feed/gain,F/G)=平均日采食量/平均日增重。

1.4.3 血清代谢指标

将收集好的血清样品解冻后,吸取500 μL于上样瓶中,使用CobasC311全自动生化分析仪进行血清代谢指标的测定。测定的血清代谢指标包括总蛋白(TP)、白蛋白(ALB)、球蛋白(GLB)、谷丙转氨酶(ALT)、谷草转氨酶(AST)、碱性磷酸酶(ALP)、乳酸脱氢酶(LDH)、淀粉酶(AMS)、血氨(NH3L)、高密度脂蛋白(HDL)、低密度脂蛋白(LDL)、甘油三酯(TG)、总胆固醇(TC)、葡萄糖(GLU)、尿素氮(UN)、总胆红素(TBIL)及C反应蛋白(CRP)。

1.4.4 血浆细胞因子含量

将收集好的血浆样本取出后,使用江苏酶免有限公司提供的酶联免疫吸附测定(ELISA)试剂盒检测血浆细胞因子含量。所测定的血浆细胞因子包括白细胞介素-1β(IL-1β)、白细胞介素-2(IL-2)、肿瘤坏死因子-α(TNF-α)、转化生长因子-β(TGF-β)、肝细胞生长因子(HGF)、血管内皮细胞生长因子(VEGF)及胰岛素样生长因子-1(IGF-1)。

1.4.5 肝脏抗氧化指标

肝脏组织匀浆上清液使用干冰保存邮寄至杭州联川生物技术服务公司检测抗氧化指标。所测肝脏抗氧化指标包括总抗氧化能力(T-AOC)、超氧化物歧化酶(SOD)、过氧化氢酶(CAT)、谷胱甘肽过氧化物酶(GSH-Px)及丙二醛(MDA)。

1.4.6 肝脏代谢相关基因相对表达量

肝脏代谢相关基因果糖双磷酸酶1(FBP1)、磷酸烯醇丙酮酸羧激酶2(PCK2)、葡萄糖-6-磷酸酶催化亚基(G6PC)、乙醛脱氢酶3家族成员A2(ALDH3A2)、乙酰辅酶A酰基转移酶1(ACAA1)、琥珀酸脱氢酶复合物亚基C(SDHC)、异柠檬酸脱氢酶3β亚基(IDH3B)、琥珀酸脱氢酶复合物亚基B(SDHB)、脂肪酸合成酶(FAS)基因表达的检测按照TaKaRa公司的RNA提取、cDNA反转录和荧光定量试剂盒说明书步骤进行,相关基因序列参考NCBI所提供的绵羊参考序列,使用Primer Premier 5.0软件进行引物设计,引物信息见表3。以甘油醛-3-磷酸脱氢酶(GAPDH)为内参基因,采用2-ΔΔCt[19]计算肝脏代谢相关基因的相对表达量。
表3 引物信息

Table 3 Primer information

基因名称
Gene names
登录号
Accession No.
引物序列
Primer sequence (5'—3')
产物大小
Product size/bp
果糖双磷酸酶1
FBP1
XM_004004092.4 F:GTCAAAGCCATCTCCAC
R:TCCCGTCACATTCGTAG
81
磷酸烯醇丙酮酸羧激酶2
PCK2
XM_015096868.2 F:GCCGTAGACCCAAAGGA
R:CGCCCAAAGTTGTAGCC
172
葡萄糖-6-磷酸酶催化亚基
G6PC
XM_004012951.4 F:AAGCCAAGCGAAGC
R:CGAAACGGGAACGA
166
乙醛脱氢酶3家族成员A2
ALDH3A2
XM_027974821.1 F:GCCGTTGTCAATGGTGGT
R:CGGTGTTTCCCGTGTAGAG
82
乙酰辅酶A酰基转移酶1
ACAA1
XM_004018227.4 F:GACAAGGGCACAGAGCA
R:TTCCAGCCGTGGTAGAG
124
琥珀酸脱氢酶复合物亚基C
SDHC
XM_004002697.3 F:GGTATTGCCTTGAGTGC
R:AGTAAGAACCAGGACAGC
255
异柠檬酸脱氢酶3β亚基
IDH3B
XM_004014386.4 F:GCAGTGGGCAGGAAT
R:TGTGAGGTTGGAGGGA
245
琥珀酸脱氢酶复合物亚基B
SDHB
XM_027965666.1 F:ATTCCACCCTGACCTTC
R:GAGCCCATCCAGTTTCT
299
脂肪酸合成酶
FASN
XM_027974304.1 F:TCCTCTGCCACTGTCTATAA
R:CCTCGAATACTACAGGTGTG
178
甘油醛-3-磷酸脱氢酶
GAPDH
AJ431207.1 F:TTCCACGGCACAGTCAAG
R:TACTCAGCACCAGCATCACC
116

1.5 数据分析

试验数据用Excel 2019进行初步整理计算后,采用SPSS 23.0统计软件进行单因素方差分析(one-way ANOVA),并用Duncan氏法进行多重比较,结果用平均值和均值标准误表示。采用GraphPad Prism软件制作图表。当P≤0.05时表示差异显著,当P>0.05时表示差异不显著。

2 结果与分析

2.1 不同比例水飞蓟粕替代豆粕对羔羊生长性能的影响

表4可知,羔羊初始体重各组之间差异不显著(P>0.05);试验结束后,羔羊的终末体重、平均日采食量、平均日增重、料重比各组之间差异均不显著(P>0.05),但值得注意的是,随着水飞蓟粕替代豆粕比例的增加,羔羊的平均日采食量呈现下降趋势,但终末体重则呈现上升趋势。
表4 不同比例水飞蓟粕替代豆粕对羔羊生长性能的影响

Table 4 Effects of different proportions of milk thistle meal instead of soybean meal on growth performance of lambs

项目
Items
组别 Groups 均值标准误
SEM
P
P-value
初始体重 IBW/kg 21.09 21.17 22.00 0.26 0.307
终末体重 FBW/kg 31.61 32.31 32.92 0.39 0.398
平均日采食量 ADFI/(kg/d) 1.29 1.26 1.22 0.02 0.477
平均日增重 ADG/(kg/d) 0.167 0.174 0.173 0.006 0.771
料重比 F/G 8.20 7.76 7.48 0.18 0.272

同行数据肩标无字母或相同小写字母表示差异不显著(P>0.05),不同小写字母表示差异显著(P≤0.05)。下表同。

In the same row, values with the no letter or the same small letter superscripts mean no significant difference (P>0.05), and with different small letter superscripts mean significant difference (P≤0.05). The same as below.

2.2 不同比例水飞蓟粕替代豆粕对羔羊血液生化指标的影响

表5可知,Ⅰ、Ⅱ、Ⅲ组羔羊各血清代谢指标均无显著差异(P>0.05)。
表5 不同比例水飞蓟粕替代豆粕对羔羊血清代谢指标的影响

Table 5 Effects of different proportions of milk thistle meal instead of soybean meal on serum metabolic indexes of lambs

项目
Items
组别 Groups 均值标准误
SEM
P
P-value
总蛋白 TP/(g/L) 81.59 78.94 76.80 0.89 0.083
白蛋白 ALB/(g/L) 39.53 39.71 38.59 0.52 0.661
球蛋白 GLB/(g/L) 42.06 39.23 38.21 0.91 0.211
谷丙转氨酶 ALT/(U/L) 22.79 23.22 23.93 1.25 0.936
谷草转氨酶 AST/(U/L) 167.78 212.00 177.44 8.15 0.060
碱性磷酸酶 ALP/(U/L) 42.67 34.00 39.63 4.35 0.596
乳酸脱氢酶 LDH/(U/L) 816.33 794.40 772.25 20.34 0.658
葡萄糖 GLU/(mmol/L) 5.40 5.78 5.27 0.28 0.751
甘油三酯 TG/(mmol/L) 0.46 0.41 0.41 0.02 0.656
总胆固醇 TC/(mmol/L) 1.88 2.03 1.98 0.05 0.473
高密度脂蛋白 HDL/(mmol/L) 1.28 1.30 1.37 0.04 0.729
低密度脂蛋白 LDL/(mmol/L) 0.61 0.77 0.70 0.04 0.217
尿素氮 UN/(mmol/L) 9.22 9.42 9.37 0.31 0.967
淀粉酶 AMS/(U/L) 12.11 10.56 11.00 0.72 0.681
血氨 NH3L/(mol/L) 552.89 531.33 534.89 16.21 0.854
总胆红素 TBIL/(mmol/L) 3.41 3.97 3.42 0.17 0.315
C反应蛋白 CRP/(mg/L) 3.89 3.88 3.86 0.01 0.729
表6可知,与Ⅰ组相比,Ⅱ组血浆中IL-1β含量增加,但差异不显著(P>0.05),但Ⅲ组血浆中IL-1β含量较Ⅰ、Ⅱ组显著增加(P≤0.05)。Ⅱ和Ⅲ组血浆中TNF-α和TGF-β含量较Ⅰ组显著提高(P≤0.05)。Ⅲ组血浆中HGF、VEGF含量与Ⅰ组相比均显著提高(P≤0.05)。随着水飞蓟粕替代豆粕比例的增加,血浆中IL-2含量呈现上升趋势,血浆中IGF-1含量先降低后升高,但各组间差异不显著(P>0.05)。
表6 不同比例水飞蓟粕替代豆粕对羔羊血浆细胞因子含量的影响

Table 6 Effects of different proportions of milk thistle meal instead of soybean meal on plasma cytokine contents of lambs

项目
Items
组别 Groups 均值标准误
SEM
P
P-value
白细胞介素-1β IL-1β/(pg/mL) 418.06a 451.00a 546.65b 20.01 0.018
肿瘤坏死因子-α TNF-α/(pg/mL) 108.12a 146.39b 144.99b 5.48 0.002
白细胞介素-2 IL-2/(pg/mL) 683.43 738.37 788.85 19.51 0.083
转化生长因子-β TGF-β/(ng/mL) 31.21a 37.49b 39.41b 0.91 <0.001
肝细胞生长因子 HGF/(pg/mL) 1 242.97a 1345.26a 1 534.02b 44.11 0.017
血管内皮细胞生长因子 VEGF/(pg/mL) 109.26a 137.10b 132.16b 3.08 <0.001
胰岛素样生长因子-1 IGF-1/(ng/mL) 1 236.98 1 220.87 1 381.17 32.10 0.075

2.3 不同比例水飞蓟粕替代豆粕对羔羊肝脏抗氧化指标的影响

表7可知,随着水飞蓟粕替代豆粕比例的增加,肝脏中GSH-Px活性持续升高,CAT活性、MDA含量持续下降,但各组之间差异均不显著(P>0.05)。与Ⅰ组相比,Ⅲ组肝脏中T-AOC、SOD活性升高,而Ⅱ组上述指标则降低,但各组之间差异均不显著(P>0.05)。
表7 不同比例水飞蓟粕替代豆粕对羔羊肝脏抗氧化指标的影响

Table 7 Effects of different proportions of milk thistle meal instead of soybean meal on liver antioxidant indexes of lambs

项目
Items
组别 Groups 均值标准误
SEM
P
P-value
总抗氧化能力 T-AOC/(mmol/g prot) 59.77 52.49 62.89 2.78 0.308
过氧化氢酶 CAT/(U/mg prot) 39.77 34.97 31.39 2.60 0.428
超氧化物歧化酶 SOD/(U/mg prot) 368.89 268.70 373.64 24.35 0.138
丙二醛 MDA/(nmol/mg prot) 0.33 0.27 0.24 0.02 0.240
谷胱甘肽过氧化物酶
GSH-Px/(U/mg prot)
390.76 394.98 454.35 23.76 0.503

2.4 不同比例水飞蓟粕替代豆粕对羔羊肝脏代谢相关基因表达的影响

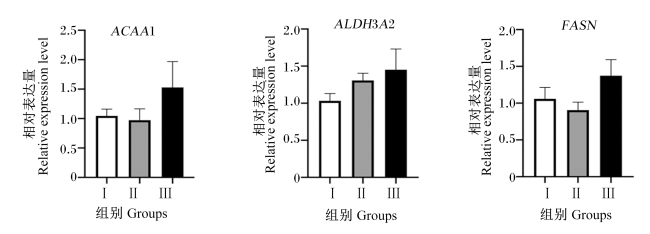
图1可知,不同比例水飞蓟粕替代豆粕对肝脏脂代谢相关基因ACAA1、ALDH3A2、FASN的相对表达量没有显著影响(P>0.05),但Ⅲ组相较Ⅰ组均有一定的上调。
图1 不同比例水飞蓟粕替代豆粕对羔羊肝脏脂代谢相关基因表达的影响

ACCA1:乙酰辅酶A酰基转移酶1 acetyl-CoA acyltransferase 1;ALDH3A2:乙醛脱氢酶3家族成员A2 aldehyde dehydrogenase 3 family member A2;FASN:脂肪酸合成酶 fatty acid synthase。

数据柱无字母标注或标注相同小写字母表示差异不显著(P>0.05),不同小写字母表示差异显著(P≤0.05)。下图同。

Fig.1 Effects of different proportions of milk thistle meal instead of soybean meal on expression of lipid metabolism related genes in liver of lambs

Data bars with no letter or the same small letters mean no significant difference (P>0.05), while with different small letters mean significant difference (P≤0.05). The same as below.

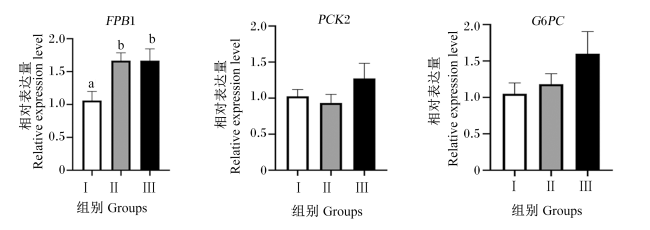
图2可知,Ⅱ、Ⅲ组羔羊肝脏糖代谢相关基因FBP1的相对表达量显著高于Ⅰ组(P≤0.05),PCK2和G6PC的相对表达量较Ⅰ组有一定的上调,但差异不显著(P>0.05)。
图2 不同比例水飞蓟粕替代豆粕对羔羊肝脏糖代谢相关基因表达的影响

FBP1:果糖双磷酸酶1 fructose-bisphosphatase 1;PCK2:磷酸烯醇丙酮酸羧激酶2 phosphoenolpyruvate carboxykinase 2;G6PC:葡萄糖-6-磷酸酶催化亚基 glucose-6-phosphatase catalytic subunit。

Fig.2 Effects of different proportions of milk thistle meal instead of soybean meal on expression of glucose metabolism related genes in liver of lambs

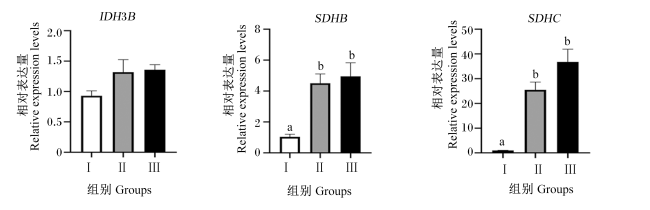
图3可知,Ⅱ、Ⅲ组羔羊肝脏三羧酸循环通路相关基因SDHBSDHC的相对表达量显著高于Ⅰ组(P≤0.05),而IDH3B的相对表达量各组之间差异不显著(P>0.05)。
图3 不同比例水飞蓟粕替代豆粕对羔羊肝脏三羧酸循环通路相关基因表达的影响

IDH3B:异柠檬酸脱氢酶3β亚基 isocitrate dehydrogenase 3β subunit;SDHB:琥珀酸脱氢酶复合物亚基B succinate dehydrogenase complex subunit B;SDHC:琥珀酸脱氢酶复合物亚基C succinate dehydrogenase complex subunit C。

Fig.3 Effects of different proportions of milk thistle meal instead of soybean meal on expression of TCA cycle pathway related genes in liver of lambs

3 讨论

3.1 不同比例水飞蓟粕替代豆粕对羔羊生长性能的影响

豆粕作为油料产品副产物,富含蛋白质,是优质蛋白质饲料原料。随着我国畜牧业快速发展以及目前国际形势的影响,农业农村部畜牧兽医局监测信息显示,豆粕价格连年持续上涨,2023年9月全国豆粕平均价格为4.93元/kg,环比上涨4.2%,青海、宁夏等地豆粕价格已至5.16元/kg。豆粕价格的持续走高已经成为制约我国畜牧业健康快速发展的重要因素,因此,新型优质蛋白质饲料开发成为解决问题的根本途径。蛋白质饲料作为饲粮中能量的重要来源,其适口性、抗营养因子含量、消化率等因素直接影响着动物的生长发育以及生产性能的好坏,替代豆粕的新型蛋白质饲料需要对针对以上问题研究后进行优选。本试验研究结果显示,饲粮中水飞蓟粕完全替代豆粕饲喂羔羊,羔羊的平均日采食量、平均日增重以及料重比等生长性能指标均与豆粕无替代组无显著差异,说明水飞蓟粕替代豆粕不会抑制羔羊的生长发育以及降低羔羊的生长性能。本试验结果与张松柏[12]、王英伟[20]的研究结果相似,他们的研究表明饲粮中水飞蓟粕替代豆粕对育肥猪以及肉牛的生长性能无显著影响,并且在降低饲料成本的情况下可以一定程度提高育肥猪胴体品质及增加肉牛过瘤胃蛋白质的质量和数量。水飞蓟粕在禽类生产中的应用研究显示,水飞蓟粕固有的抗菌性、抗氧化性和保肝作用,使得水飞蓟粕作为饲料添加剂可以提高鸡蛋品质和蛋壳强度,并且可以提高禽类肝脏的氧化稳定性,从而提高肝脏健康,但是水飞蓟粕中的粗纤维含量较高[21],限制了其在禽类饲粮中的使用比例[22],并且Kosiorowska等[23]研究指出,粗纤维含量高的饲粮会对犊牛的采食量造成影响。因此,如果对水飞蓟粕进一步加工降低粗纤维含量,增加其适口性[24-25],从而提高采食量和使用比例,可能会创造更高的经济效益。综上可知,水飞蓟粕作为替代豆粕的新型蛋白质饲料,对畜禽生长无抑制作用且无负面影响,水飞蓟粕替代豆粕可在一定程度上降低饲养成本,进而提高生产效益,对动物生产具有积极作用。

3.2 不同比例水飞蓟粕替代豆粕对羔羊血液生化指标的影响

3.2.1 不同比例水飞蓟粕替代豆粕对羔羊血清代谢指标的影响

血液中的各种中间代谢产物,如糖、脂类、酶、蛋白质等与动物的生长发育、机体营养代谢水平、生理健康等关系密切,当动物机体机能出现异常时,其血液中的代谢指标也会随之发生相应变化[26-27]。因此,通过血液代谢指标可以反映动物生理机能的状态,并进行相应的疾病诊断,从而对饲养管理进行指导来保障动物的安全生产[28]。血清总蛋白含量可以反映饲粮蛋白质水平及机体对蛋白质的代谢水平[29]。当饲粮中的蛋白质供应不足时,血液中总蛋白、白蛋白的含量就会下降[30]。肝脏是蛋白质代谢的重要器官[31],血清中转氨酶的活性是反映肝脏功能的重要指标,临床上多通过检测血清谷丙转氨酶和谷草转氨酶活性来反映肝脏健康程度[32-33]。葡萄糖是动物机体重要的能量来源之一,血液中的葡萄糖含量可直接反映机体能量平衡状态,当机体能量缺乏时,血液中葡萄糖的含量下降[34]。血液中总胆固醇和甘油三酯的含量与饲粮的营养水平密切相关,指示机体脂类代谢情况[35-38];高密度脂蛋白、低密度脂蛋白含量则反映机体对胆固醇的代谢情况[39];尿素氮含量反映动物机体蛋白质代谢和饲粮氨基酸的平衡状况以及机体对氮的利用情况[40-42];碱性磷酸酶活性反映机体对钙、磷的吸收情况并在骨骼的发育过程中发挥作用[43]。研究发现,动物的体重和C反应蛋白的含量关系密切,体重与C反应蛋白含量呈正相关,并且C反应蛋白与机体炎症具有密切相关性[44]。本试验结果显示,饲粮中水飞蓟粕完全替代豆粕饲喂羔羊,羔羊血清中各代谢指标与豆粕无替代组无显著差异,说明各组羔羊机体内各类营养物质的代谢水平未发生显著变化,水飞蓟粕用于肉羊羔羊饲养对羔羊机体及生理机能没有造成负面影响,水飞蓟粕用于羔羊生产是安全可行的。

3.2.2 不同比例水飞蓟粕替代豆粕对羔羊血浆细胞因子含量的影响

血液当中存在由免疫细胞及某些非免疫细胞分泌的一些具有生物活性的小分子多肽或糖蛋白,这些小分子蛋白质介导组织细胞间的相互作用,具有调节细胞生长、调节免疫应答或参与炎症反应的作用[45-46]。IL-1β是一种由活化的巨噬细胞产生的细胞因子,属于激素样肽类物质,刺激参与免疫反应的细胞增殖分化,并提高其功能[47]。余亚东等[48]在研究酵母培养物对犊牛机体免疫力的影响时发现,饲粮中添加酵母培养物可以提高血清中IL-1β的含量,增强了犊牛机体吞噬细胞的活性,提高了机体的非特异性免疫能力。IL-2由T细胞产生,属于T细胞生长因子,可以加强T细胞的杀伤活性,促进活化B细胞增殖,具有提高免疫力的作用。IL-1β和IL-2都属于白细胞介素,其含量高低可以反映机体的免疫水平[49]。张学峰等[50]通过对小尾寒羊灌服酵母培养物进行研究发现,灌服2.0%酵母培养物的试验组其血液中IL-2含量显著高于对照组。TNF-α是由多种细胞如巨噬细胞、淋巴细胞和嗜中性粒细胞等细胞分泌的炎性细胞因子。TNF-α可以通过调节免疫细胞发育、稳态、激活及免疫耐受的维持来启动及控制炎症反应[51]。TGF-β是一种多功能的细胞因子,可以调节多种细胞生长、分化及凋亡等;此外,TGF-β还具有重要的免疫调节作用[52]。HGF可以调节细胞的生长发育和运动,还具有抗纤维、抗细胞凋亡和促进有丝分裂等多种作用,并在肝脏实质细胞的生长发育中有重要的作用[53]。VEGF是一种具有高度特异性的可以促进血管内皮细胞进行分裂的生长因子,能够使血管的通透性增加,从而使各种营养物质及代谢产物更容易通过[54]。IGF-1主要由肝脏分泌,能够促进细胞的增殖、组织的生长发育,并能够防治多种代谢性疾病[55]。本试验结果表明,水飞蓟粕完全替代豆粕饲喂羔羊,羔羊血浆中的免疫相关细胞因子IL-1β、TNF-α、TGF-β、HGF、VEGF的含量均显著升高,IL-2和IGF-1的含量有升高趋势,说明水飞蓟粕替代豆粕饲喂羔羊使羔羊免疫细胞因子处于活跃状态,这可能与水飞蓟粕中含有一定量的水飞蓟素有关,水飞蓟素具有抗氧化、抗炎、免疫调节的作用,并具有保肝护肝以及治疗肝炎的效果[56-58]。陈刚等[59]在研究水飞蓟素对石斑鱼血清生化指标、脂代谢相关基因表达及肝脏代谢组的影响时发现,水飞蓟素具有抗氧化和免疫调节作用。蔡龙等[60]的研究显示,水飞蓟素可以作为抗生素替代物发挥作用,促进畜禽生长并保护畜禽健康。因此,水飞蓟粕作为新型蛋白质饲料替代豆粕使用还需要对其具体的营养成分和潜在的药代动力学进行研究,从而更加科学地指导水飞蓟粕在畜禽生产中的使用。

3.3 不同比例水飞蓟粕替代豆粕对羔羊肝脏抗氧化能力的影响

水飞蓟粕是水飞蓟籽提取水飞蓟素后剩余的残渣,含有丰富的黄酮类物质,具有与水飞蓟素相似的抗氧化作用[61]。机体内自由基维持平衡状态主要依赖抗氧化系统,当机体产生内源性氧自由基时,则发生氧化应激反应,此时机体通过抗氧化系统来清除这些自由基,重新形成自由基的平衡状态[62]。T-AOC可以从整体上反映出机体的抗氧化能力,SOD[63]、CAT[64]以及GSH-Px是机体抗氧化系统内的3种抗氧化酶,可以清除对机体有害的超氧阴离子等自由基,从而避免机体的氧化损伤。MDA是机体脂质过氧化的产物,其含量可以反映出机体受自由基攻击的严重程度[65]。因此,检测肝脏中SOD、CAT、GSH-Px的活性以及MDA的含量可以反映出肝脏的氧化应激水平和损伤程度[66]。朱淑云等[67]的研究发现,水飞蓟素能够显著提高小鼠血清中SOD、GSH-Px的活性和T-AOC。Kiruthiga等[68]报道,水飞蓟素可以提高因过氧化氢(H2O2)浓度升高所导致的SOD和GSH-Px活性的下降以及MDA含量的升高。本研究结果表明,当水飞蓟粕完全替代豆粕时,羔羊肝脏中SOD和GSH-Px活性和T-AOC上升,而CAT活性、MDA含量则下降。羔羊肝脏SOD和GSH-Px活性和T-AOC上升可能是水飞蓟粕中依然含有一定量的水飞蓟素,从而提高羔羊肝脏的抗氧化能力。王红军等[69]通过对水飞蓟素抗氧化的机制进行研究发现,当机体的氧化应激源为羟自由基(·OH)形式时,水飞蓟素可以直接通过理化作用来清除·OH,并抑制机体的脂质过氧化反应,从而减少MDA的产生;当机体的氧化应激为超氧阴离子自由基( O 2 -·)或H2O2形式时,水飞蓟素可以清除 O 2 -·或由H2O2所产生的·OH,但对H2O2本身没有太大作用。本试验中水飞蓟粕代替豆粕使羔羊肝脏MDA含量下降,也同样说明水飞蓟粕具有提高机体抗氧化性,减少氧化应激损伤的作用,而造成肝脏CAT活性下降,可能是因为水飞蓟粕和水飞蓟素一样是通过清除 O 2 -·或·OH来起作用的,而CAT主要是通过分解H2O2来起作用,所以添加水飞蓟粕没有使CAT活性上升,但造成其下降的具体原因尚不清楚,还有待进一步研究。本研究中羔羊肝脏抗氧化指标各组间的差异均没达到显著水平,可能是由于水飞蓟粕中含有的水飞蓟素较少以及试验动物为幼龄动物其自身的抗氧化性较强的原因所致[70]。从试验结果来看,水飞蓟粕替代豆粕有提高羔羊肝脏抗氧化能力的趋势,水飞蓟粕添加到饲粮中可以在一定程度上提高机体的抗氧化能力,但抗氧化效果与添加比例以及试验条件等因素有关。

3.4 不同比例水飞蓟粕替代豆粕对羔羊肝脏代谢相关基因表达的影响

肝脏是物质在机体内代谢的主要器官,是脂肪、糖、氨基酸等代谢的主要场所,肝脏代谢水平一定程度上代表机体代谢水平,肝脏代谢平衡,则机体健康稳定[71]。脂肪是动物机体供热的主要来源,主要以甘油三酯和脂肪酸的形式参与机体代谢。肝脏是脂肪酸合成和分解的重要场所,脂肪被水解为游离脂肪酸和甘油三酯,游离脂肪酸被血液运输到肝脏进入线粒体,在线粒体内经过氧化磷酸化和三羧酸循环途径后被彻底氧化成二氧化碳和水并释放大量的ATP,给机体提供能量[72]。脂肪酸是维持动物机体健康的重要营养成分之一,并且脂肪酸与肉品质关系紧密[73]。ACAA1在动物的不饱和脂肪酸合成和代谢中发挥着重要的作用[74],是调控过氧化物酶体增殖物激活受体(PPAR)途径下游脂肪酸合成和转运过程中关键的酶。王延莉等[75-76]研究发现,绵羊ACAA1不同基因型与肉品质具有相关性,并且直接参与调控脂肪酸代谢。Wang等[77]依据研究结果推测ACAA1是脂类代谢中的关键基因。ALDH3A2参与肝脏脂代谢,通过催化中等长度的饱和及不饱和脂肪醛氧化为脂肪酸,将脂肪酸转化为能量被机体利用[78]。FASN负责催化乙酰辅酶A(acetyl-CoA)和丙二酰辅酶A(malonyl-CoA)合成16碳的棕榈酸,进而生成棕榈油酸,参与肝脏脂代谢过程[79]。肝脏脂代谢对机体供能及健康至关重要,但目前有关水飞蓟粕对羊肝脏脂代谢的影响未见报道。本研究发现,水飞蓟粕替代豆粕对羔羊肝脏脂代谢相关基因ACAA1、ALDH3A2、FASN的表达具有一定上调作用,但还未达到显著水平,当饲粮中水飞蓟粕完全替代豆粕时,可以在一定程度上提高羔羊肝脏中脂肪酸的合成速率,更多的脂肪酸可以通过β-氧化生成乙酰辅酶A进入三羧酸循环,给机体生长提供更多的能量。由此推测,水飞蓟粕替代豆粕可以在一定程度上促进肝脏脂代谢,产生更多能量提供机体生长发育。
葡萄糖是动物机体供能的主要来源,肝脏是调节血糖水平的主要器官,肝脏的糖代谢主要是肝糖原合成分解和糖异生作用。FBP1、PCK2、G6PC均在肝脏糖代谢过程中发挥重要调控作用[80-82]。本研究发现,水飞蓟粕完全替代豆粕,羔羊肝脏中糖代谢相关基因FBP1的相对表达量显著上调,PCK2和G6PC的相对表达量有上调趋势,表明水飞蓟粕可以通过对糖代谢相关基因的表达进行上调来促进肝脏中糖代谢限速酶的活性,从而提高肝脏功能,提高肝脏调节血糖平衡的能力,产生更多能量给机体供能。
动物所需的三大营养物质糖类、脂类和氨基酸代谢的交汇通路是线粒体内的三羧酸循环,三羧酸循环是三大物质代谢联系的枢纽[83]。异柠檬酸脱氢酶(IDH)、琥珀酸脱氢酶(SDH)是三羧酸循环通路内的关键限速酶[84]。IDH3B主要位于线粒体内,功能是将NAD+/NADP+还原为NADH/NADPH,为细胞提供能量和生物合成前体物质[85]。SDH是位于线粒体内膜上的一种膜结合酶,在细胞的能量代谢中发挥着重要的作用,是反映机体有氧代谢的重要限速酶,是线粒体的标志酶,其活性是评价三羧酸循环程度的指标,SDH有SDHA、SDHB、SDHC和SDHD 4个亚基,其中SDHB为亲水性催化亚基,SDHC为疏水性催化亚基,SDHB可以催化琥珀酸氧化生成延胡索酸[86]。本研究发现,水飞蓟粕完全替代豆粕可以显著上调羔羊肝脏细胞内三羧酸循环限速酶编码基因SDHBSDHC的相对表达量,对IDH3B的相对表达量有上调趋势,表明水飞蓟粕代替豆粕可以促进肝脏内三羧酸循环和氧化磷酸化的进程,加快肝脏能量代谢速率,为动物机体生长发育以及抗寒提供更多能量。

4 结论

生长性能结果显示,水飞蓟粕对羔羊生长无抑制作用;血液生化指标结果显示,水飞蓟粕对羔羊生理机能无不良影响,同时可以提高血液中免疫细胞因子含量,有助于提高羔羊抗病性;肝脏抗氧化指标结果显示,水飞蓟粕有改善羔羊肝脏抗氧化能力的趋势;肝脏代谢相关基因表达结果显示,水飞蓟粕可以上调羔羊肝脏代谢相关基因表达,促进肝脏糖、脂代谢,加快能量代谢循环。综上所述,羔羊饲粮中使用水飞蓟粕替代豆粕是安全可行的,且可以提高肝脏抗氧化能力,有助于提高羔羊抗病性,并加快肝脏能量代谢循环速率,对羔羊生产具有积极作用。
[1]
贺泽霖, 陈晶, 倪洪涛, 等. 药用植物水飞蓟的研究进展[J]. 中国农学通报, 2022, 38(18):128-132.

DOI

HE Z L, CHEN J, NI H T, et al. Medicinal plant resource Silybum marianum L.Gaertn:a review[J]. Chinese Agricultural Science Bulletin, 2022, 38(18):128-132. (in Chinese).

[2]
SALIH M J, HADI T A. Effect of adding milk thistle Silybum marianum cereal to ration on performance of productive and physiological of laying hens[J]. IOP Conference Series:Earth and Environmental Science, 2023, 1225(1):012045.

DOI

[3]
MAHGOUB Y A, SHAWKY E, GHAREEB D A, et al. UPLC-MS/MS multivariate data analysis reveals phenological growth stages affect silymarin bioactive components of the different organs of two Silybum marianum genotypes[J]. Microchemical Journal, 2023, 187:108436.

DOI

[4]
BENCZE-NAGY J, STRIFLER P, HORVÁTH B, et al. Effects of dietary milk thistle (Silybum marianum) supplementation in ducks fed mycotoxin-contaminated diets[J]. Veterinary Sciences, 2023, 10(2):100.

DOI

[5]
MAGDALENA K, DOROTA G, GRETA A. The effect of milk thistle (Silybum marianum L.) fortification,rich in dietary fibre and antioxidants,on structure and physicochemical properties of biscuits[J]. Applied Sciences, 2022, 12(23):12501.

DOI

[6]
GILABADI S, STANYON H, DECEITA D, et al. Simple and effective method for the extraction of silymarin from Silybum marianum (L.) gaertner seeds[J]. Journal of Herbal Medicine, 2023, 37:100619.

DOI

[7]
SADOWSKA K, ANDRZEJEWSKA J, LIGOCKA A, et al. Bioactive substances and microbiological quality of milk thistle fruits from organic and conventional farming[J]. Applied Sciences, 2023, 13(14):8536.

DOI

[8]
杨明, 丁立威. 水飞蓟产销历史、现状与后市分析[J]. 特种经济植物, 2013(3):19-22.

YANG M, DING L W. History,current situation,and future market analysis of silymarin production and marketing[J]. Special Economic Animal and Plant, 2013(3):19-22. (in Chinese)

[9]
RACLARIU-MANOLICǍ A C, SOCACIU C. Detecting and profiling of milk thistle metabolites in food supplements:a safety-oriented approach by advanced analytics[J]. Metabolites, 2023, 13(3):440.

DOI

[10]
高建绪, 马浩凯, 刘蕊, 等. 水飞蓟粕利用现状及开发进展[J]. 黑龙江畜牧兽医, 2023(3):36-40.

GAO J X, MA H K, LIU R, et al. Utilization status and development progress of milk thistle meal[J]. Heilongjiang Animal Science and Veterinary Medicine, 2023(3):36-40. (in Chinese)

[11]
杨航, 杨桂芹, 赵辉. 水飞蓟粕在动物生产上的利用现状及前景[J]. 黑龙江农业科学, 2016(12):151-154.

YANG H, YANG G Q, ZHAO H. Utilization status and prospect of Silybum marianum meal in animal production[J]. Heilongjiang Agricultural Sciences, 2016(12):151-154. (in Chinese)

[12]
张松柏. 水飞蓟粕在肉牛中的开发利用及机理研究[D].硕士学位论文. 福州: 福建农林大学, 2011.

ZHANG S B. The study of utilization and mechenism of milk thistle cake in beef production.[D].Master’s Thesis. Fuzhou: Fujian Agriculture and Forestry University, 2011. (in Chinese)

[13]
孙婷婷, 张雨, 战皓宇, 等. 水飞蓟粕替代豆粕饲喂獭兔的应用研究[J]. 吉林农业科技学院学报, 2014, 23(4):1-4.

SUN T T, ZHANG Y, ZHAN H Y, et al. Research on application of milk thistle meal instead of soybean meal feeding rex rabbit[J]. Journal of Jilin Agricultural Science and Technology College, 2014, 23(4):1-4. (in Chinese)

[14]
吴峰洋, 李冲, 陈赛娟, 等. 红花粕和水飞蓟粕对生长獭兔的营养价值评定[J]. 动物营养学报, 2017, 29(2):663-669.

WU F Y, LI C, CHEN S J, et al. Nutritional value evaluation of safflower meal and milk thistle meal for growing Rex rabbits[J]. Chinese Journal of Animal Nutrition, 2017, 29(2):663-669. (in Chinese)

[15]
VOJTÍSEK B, HRONOVÁ B, HAMRÍK J. [Milk thistle (Silybum marianum,L.,Gaertn.) in the feed of ketotic cows][J]. Veterinarni Medicina, 1991, 36(6):321-330.

[16]
LI F, LI F, ZHAO T, et al. Solid-state fermentation of industrial solid wastes from the fruits of milk thistle Silybum marianum for feed quality improvement[J]. Applied Microbiology and Biotechnology, 2013, 97(15):6725-6737.

DOI

[17]
HASHEMI J N S, MAHDAVI A H, ANSARI M S, et al. Effects of milk thistle meal on performance,ileal bacterial enumeration,jejunal morphology and blood lipid peroxidation in laying hens fed diets with different levels of metabolizable energy[J]. Journal of Animal Physiology and Animal Nutrition, 2018, 102(2):410-420.

DOI

[18]
熊本海, 罗清尧, 郑姗姗, 等. 中国饲料成分及营养价值表 (2020年第31版) 制订说明[J]. 中国饲料, 2020(21):87-97.

XIONG B H, LUO Q Y, ZHENG S S, et al. Introduction of tables of feed composition and nutritive values in China (2020 thirty-first edition)[J]. China Feed, 2020(21):87-97. (in Chinese)

[19]
SCHMITTGEN T D, LIVAK K J. Analyzing real-time PCR data by the comparative C (T) method[J]. Nature Protocols, 2008, 3(6):1101-1108.

DOI

[20]
王英伟. 水飞蓟残渣在育肥猪生产上的应用[D].硕士学位论文. 延吉: 延边大学, 2006.

WANG Y W. Application of silymarin residue in the production of fattening pigs[D].Master’s Thesis. Yanji: Yanbian University, 2006. (in Chinese)

[21]
李峰. 药渣水飞蓟粕固态发酵生产生物蛋白饲料的研究与应用[D].硕士学位论文. 镇江: 江苏大学, 2012.

LI F. Research and application of solid-state fermentation of medicinal residue and silymarin meal to produce biological protein feed[D].Master’s Thesis. Zhenjiang: Jiangsu University, 2012. (in Chinese)

[22]
VARASTEGANI A, ISMAIL D. Influence of dietary fiber levels on feed utilization and growth performance in poultry[J]. Journal of Animal Production Advances, 2014, 4:422-429.

[23]
KOSIOROWSKA A, PUGGAARD L, HEDEMANN M S, et al. Gastrointestinal development of dairy calves fed low-or high-starch concentrate at two milk allowances[J]. Animal:an International Journal of Animal Bioscience, 2011, 5(2):211-219.

DOI

[24]
LIU Y X, WU M H, REN M M, et al. From medical herb to functional food:development of a fermented milk containing silybin and protein from milk thistle[J]. FOODS, 2023, 12(6):1308.

DOI

[25]
PEREIRA I C, COSTA C F, MARTINS C L, et al. Voluntary daily fluctuation in dry matter intake is associated to feedlot performance,feeding behavior and rumen morphometrics in beef cattle[J]. Livestock Science, 2021, 250:104565.

DOI

[26]
MO J Y, LU Y J, XING T Q, et al. Blood metabolic and physiological profiles of Bama miniature pigs at different growth stages[J]. Porcine Health Management, 2022, 8(1):35.

DOI PMID

[27]
GAO J, YANG D Y, SUN Z Y, et al. Changes in blood metabolic profiles reveal the dietary deficiencies of specific nutrients and physiological status of grazing yaks during the cold season in Qinghai Province of China[J]. Metabolites, 2022, 12(8):738.

DOI

[28]
PICCIONE G, CASELLA S, LUTRI L, et al. Reference values for some haematological,haematochemical,and electrophoretic parameters in the Girgentana goat[J]. Turkish Journal of Veterinary and Animal Sciences, 2010, 34(2):197-204.

[29]
萧培珍, 吉红, 张宝彤, 等. 水飞蓟素抑制草鱼肝细胞脂质蓄积的作用及其机制研究[J]. 水生生物学报, 2017, 41(6):1301-1310.

XIAO P Z, JI H, ZHANG B T, et al. Inhibitory effect of silymarin on oleic acid-induced lipid accumulation in grass carp (Ctenopharyngodon idellus) hepatocytes in vitro[J]. Acta Hydrobiologica Sinica, 2017, 41(6):1301-1310. (in Chinese)

[30]
KASSAB A Y, SOLIMAN E B, MOTY A K I A E, et al. Productive performance and blood metabolites as affected by protected protein in sheep[J]. Open Journal of Animal Sciences, 2011, 1:24-32.

DOI

[31]
OPGENORTH J, ABUAJAMIEH M, HORST E A, et al. The effects of zinc amino acid complex on biomarkers of gut integrity,inflammation,and metabolism in heat-stressed ruminants[J]. Journal of Dairy Science, 2020, 104(2):2410-2421.

DOI

[32]
WANG S J, YAN M, TIAN W, et al. Industry-produced and ruminant-derived trans-fatty acids and subclinical myocardial injury in adults without known cardiovascular disease[J]. Journal of Internal Medicine, 2023, 294(6):816-818.

DOI

[33]
TIMMERMAN H M, KONING C J M, MULDER L, et al. Monostrain,multistrain and multispecies probiotics—a comparison of functionality and efficacy[J]. International Journal of Food Microbiology, 2004, 96(3):219-233.

DOI

[34]
GAO L M, LIU G Y, WANG H L, et al. Maternal pyrimidine nucleoside supplementation regulates fatty acid,amino acid and glucose metabolism of neonatal piglets[J]. Animal Nutrition, 2022, 11:309-321.

DOI

[35]
GHAVIPANJE N, FATHI NASRI M H, FARHANGFAR S H, et al. Regulation of nutritional metabolism in transition dairy goats:energy balance,liver activity,and insulin resistance in response to berberine supplementation[J]. Animals, 2021, 11(8):2236.

DOI

[36]
DOS SANTOS COSTA C, ROGÉRIO M C P, FERREIRA A L, et al. Dietary nutrient restrictions in the post-weaning period change Santa Inês ewe lamb nutritional metabolic profile[J]. Tropical Animal Health and Production, 2021, 53(3):359.

DOI PMID

[37]
JIAO D, LIANG Y P, ZHOU S S, et al. Supplementing diets with Agriophyllum squarrosum reduced blood lipids,enhanced immunity and anti-inflammatory capacities,and mediated lipid metabolism in tan lambs[J]. Animals, 2022, 12(24):3486.

DOI

[38]
蔡珣. TMR技术对奶牛生产性能及部分血液生化指标影响的研究[D].硕士学位论文. 武汉市: 华中农业大学, 2005.

CAI X. Effects of total mixed ration technique on production performance and some blood biochemical indexes of dairy cows[D].Master’s Thesis. Wuhan: Huazhong Agricultural University, 2005. (in Chinese)

[39]
REISINGER A C, SCHULLER M, SOURIJ H, et al. Impact of sepsis on high-density lipoprotein metabolism[J]. Frontiers in Cell and Developmental Biology, 2021, 9:795460.

DOI

[40]
NIYIGENA V, COFFEY K P, COBLENTZ W K, et al. Nitrogen balance and blood urea nitrogen by gestating sheep offered alfalfa silage wrapped with or without an enhanced oxygen barrier plastic after time delays up to three days[J]. Small Ruminant Research, 2021, 198:106355.

DOI

[41]
ADIWINARTI R, KUSTANTINAH, BUDISATRIA I G S, et al. Profile of rumen fermentation and blood urea nitrogen concentration of Kacang goat fed total mixed ration vs.roughage[J]. IOP Conference Series:Earth and Environmental Science, 2018, 119:012049.

DOI

[42]
STEPHENSON E, MEYER A, RADUNZ A. Effects of protein supplementation on beef heifer circulating non-esterified fatty acids,blood urea nitrogen (BUN),and glucose in relation to time of feeding[J]. Journal of Animal Science, 2018, 96(S3)440-441.

[43]
FERNANDEZ N J, KIDNEY B A. Alkaline phosphatase:beyond the liver[J]. Veterinary Clinical Pathology, 2007, 36(3):223-233.

DOI

[44]
PEPYS M B, HIRSCHFIELD G M, et al. C-reactive protein:a critical update[J]. The Journal of Clinical Investigation, 2003, 111(12):1805-1812.

DOI

[45]
YALTA T, YALTA K. Systemic inflammation and arrhythmogenesis:a review of mechanistic and clinical perspectives[J]. Angiology, 2018, 69(4):288-296.

DOI

[46]
PARDOLL D M. Spinning molecular immunology into successful immunotherapy[J]. Nature Reviews Immunology, 2002, 2(4):227-238.

DOI PMID

[47]
ABDEL-FATTAH A, ABDELWAHAB M G. Interleukin-1β,tumor necrosis factor-α,and oxidative stress biomarkers in cows with acute Brucella abortus infection[J]. Comparative Clinical Pathology, 2021, 30:311-315.

DOI

[48]
余亚东. 酵母培养物添加方式对哺乳期犊牛生长发育与机体免疫力的影响[D].硕士学位论文. 银川: 宁夏大学, 2017.

YU Y D. Effects of different addition ways of yeast culture on growth performance and immune function of calves in suckling period[D].Master’s Thesis. Yinchuan: Ningxia University, 2017. (in Chinese)

[49]
MARTINS R P, SOUZA F N. Editorial:cell-mediated immunity in ruminants:novel approaches and insights[J]. Frontiers in Veterinary Science, 2023, 10:1177315.

DOI

[50]
张学峰, 王兰惠, 周雪飞, 等. 瘤胃灌注酵母培养物对绵羊血液生化指标和免疫及抗氧化功能的影响[J]. 中国畜牧杂志, 2016, 52(9):62-65.

ZHANG X F, WANG L H, ZHOU X F, et al. Effects of rumen infusion of yeast culture on blood biochemical indicators,immune and antioxidant functions in sheep[J]. Chinese Journal of Animal Science, 2016, 52(9):62-65. (in Chinese)

[51]
MOREIRA T P, DE SOUSA C D F, DE MELO COSTA V R, et al. Tumour necrosis factor plays a deleterious role in the pathogenesis of Chikungunya virus infection[J]. Immunology, 2023, 168(3):444-458.

DOI

[52]
KHAN M Z, LIU S, MA Y L, et al. Overview of the effect of rumen-protected limiting amino acids (methionine and lysine) and choline on the immunity,antioxidative,and inflammatory status of periparturient ruminants[J]. Frontiers in Immunology, 2023, 13:1042895.

DOI

[53]
YAN L T, HE X X, TANG Y H, et al. HGF can reduce accumulation of inflammation and regulate glucose homeostasis in T2D mice[J]. Journal of Physiology and Biochemistry, 2021, 77(4):614-624.

[54]
WANG C G, LOU Y T, TONG M J, et al. Author correction:asperosaponin Ⅵ promotes angiogenesis and accelerates wound healing in rats via up-regulating HIF-1α/VEGF signaling[J]. Acta Pharmacologica Sinica, 2022, 43(6):1617-1618.

DOI

[55]
ORRÙ S, NIGRO E, MANDOLA A, et al. A functional interplay between IGF-1 and adiponectin[J]. International Journal of Molecular Sciences, 2017, 18(10):2145.

DOI

[56]
FRASCHINI F, DEMARTINI G, ESPOSTI D. Pharmacology of silymarin[J]. Clinical Drug Investigation, 2002, 22:51-65.

DOI

[57]
FAN L, MA Y L, LIU Y, et al. Silymarin induces cell cycle arrest and apoptosis in ovarian cancer cells[J]. European Journal of Pharmacology, 2014, 743:79-88.

DOI PMID

[58]
GILLESSEN A, SCHMIDT H H J. Silymarin as supportive treatment in liver diseases:a narrative review[J]. Advances in Therapy, 2020, 37(4):1279-1301.

DOI

[59]
陈刚, 欧光海, 温震威, 等. 水飞蓟素对杂交石斑鱼幼鱼血清生化指标、脂代谢相关基因表达及肝脏代谢组的影响[J]. 广东海洋大学学报, 2023, 43(4):41-51.

CHEN G, OU G H, WEN Z W, et al. Effects of dietary silymarin supplementation on serum biochemical parameters,lipid metabolism-related gene expression,and liver metabolome in juvenile hybrid grouper (Epinephelus fuscoguttatus♀×Epinephelus polyphekadion ♂)[J]. Journal of Guangdong Ocean University, 2023, 43(4):41-51. (in Chinese)

[60]
蔡龙, 蒋显仁, 丁宏标, 等. 水飞蓟素的生物学功能及其在畜禽生产中的应用研究进展[J]. 中国畜牧杂志, 2023, 59(1):27-34.

CAI L, JIANG X R, DING H B, et al. Biological functions of silymarin and its application in livestock and poultry production[J]. Chinese Journal of Animal Science, 2023, 59(1):27-34. (in Chinese)

[61]
张娟, 白庆云, 田丽莉. 水飞蓟素防治实验性肝病的作用及相关临床应用的研究进展[J]. 中国现代应用药学, 2023, 40(19):2745-2753.

ZHANG J, BAI Q Y, TIAN L L. Research progress on the effects of silymarin against experimental liver disease and related clinical application[J]. Chinese Journal of Modern Applied Pharmacy, 2023, 40(19):2745-2753. (in Chinese)

[62]
FINKEL T, HOLBROOK N J. Oxidants,oxidative stress and the biology of ageing[J]. Nature, 2000, 408(6809):239-247.

DOI

[63]
HOLDOM M D, LECHENNE B, HAY R J, et al. Production and characterization of recombinant Aspergillus fumigatus Cu,Zn superoxide dismutase and its recognition by immune human sera[J]. Journal of Clinical Microbiology, 2000, 38(2):558-562.

DOI

[64]
TANG M H, FANG R J, XUE J J, et al. Effects of catalase on growth performance,antioxidant capacity,intestinal morphology,and microbial composition in yellow broilers[J]. Frontiers in Veterinary Science, 2022, 9:802051.

DOI

[65]
KONG X F, WU G Y, LIAO Y P, et al. Effects of Chinese herbal ultra-fine powder as a dietary additive on growth performance,serum metabolites and intestinal health in early-weaned piglets[J]. Livestock Science, 2007, 108(1/2/3):272-275.

DOI

[66]
SIMÕES-ALVES A C, COSTA-SILVA J H, BASSOT A, et al. Diet enriched in saturated fatty acids induces liver oxidative stress and elicits inflammatory pathways prior to metabolic disruption in perinatal protein undernutrition[J]. Nutrition Research(New York,N.Y.), 2023, 118:104-115.

[67]
朱淑云, 周越, 肖香, 等. 水飞蓟油的体外抗氧化活性及对氧化损伤小鼠的保护作用[J]. 食品科学, 2018, 39(5):234-238.

DOI

ZHU S Y, ZHOU Y, XIAO X, et al. Antioxidant activity in vitro of Silybum marianum seed oil and its protective effect on oxidative damage in mice[J]. Food Science, 2018, 39(5):234-238. (in Chinese)

DOI

[68]
KIRUTHIGA P V, SHAFREEN R B, PANDIAN S K, et al. Silymarin protection against major reactive oxygen species released by environmental toxins:exogenous H2O2 exposure in erythrocytes[J]. Basic & Clinical Pharmacology & Toxicology, 2007, 100(6):414-419. (in Chinese)

[69]
王红军, 姜媛媛, 路平, 等. 水飞蓟宾的抗肿瘤、抗氧化和免疫调节分子药理学机制研究进展[J]. 药学学报, 2010, 45(4):413-421.

WANG H J, JIANG Y Y, LU P, et al. An updated review at molecular pharmacological level for the mechanism of anti-tumor,antioxidant and immunoregulatory action of silibinin[J]. Acta Pharmaceutica Sinica, 2010, 45(4):413-421. (in Chinese)

[70]
马作霖. 乳清粉调节D-半乳糖诱导衰老小鼠肠道菌群结构及抗衰老作用研究[D].博士学位论文. 兰州: 甘肃农业大学, 2021.

MA Z L. A study on intestinal microflora structure regulation and anti-aging effect of whey powder in D-galactose induced aging mice[D].Ph.D.Thesis. Lanzhou: Gansu Agricultural University, 2021. (in Chinese)

[71]
郭鹏程. 利用时空多组学解析肝脏功能结构及肝再生、肝纤维化分子机制的研究[D].博士学位论文. 长春: 吉林大学, 2023.

GUO P C. High-definition spatial transcriptomic atlas reveals new principle of liver homeostasis,regeneration and fibrosis[D].Ph.D.Thesis. Changchun: Jilin University, 2023. (in Chinese)

[72]
GLATZ J F C, LUIKEN J J F P, BONEN A. Membrane fatty acid transporters as regulators of lipid metabolism:implications for metabolic disease[J]. Physiological Reviews, 2010, 90(1):367-417.

DOI

[73]
陈佳亿. 不同营养水平日粮对宁乡猪生长性能、胴体性状及肉品质的影响[D].博士学位论文. 长沙: 湖南农业大学, 2021.

CHEN J Y. Effects of different nutrition levels dietary on growth performance,carcass traits and meat quality of Ningxiang pigs[D].Ph.D.Thesis. Changsha: Hunan Agricultural University, 2021. (in Chinese)

[74]
HUNT M C, SIPONEN M I, ALEXSON S E H. The emerging role of acyl-CoA thioesterases and acyltransferases in regulating peroxisomal lipid metabolism[J]. Biochimica et Biophysica Acta, 2012, 1822(9):1397-1410.

DOI PMID

[75]
王延莉, 曹阳, 梁祎凡, 等. 乙酰辅酶A酰基转移酶1基因研究进展[J]. 中国畜牧杂志, 2019, 55(10):42-46.

WANG Y L, CAO Y, LIANG Y F, et al. Advance in acetyl-CoA acyltransferase 1 gene[J]. Chinese Journal of Animal Science, 2019, 55(10):42-46. (in Chinese)

[76]
王延莉, 曹阳, 梁祎凡, 等. 绵羊ACAA1基因多态性及其与肉质性状的关联性分析[J]. 吉林农业大学学报, 2022, 44(2):204-209.

WANG Y L, CAO Y, LIANG Y F, et al. Polymorphism of ACAA1 gene and its association with meat quality trait in sheep[J]. Journal of Jilin Agricultural University, 2022, 44(2):204-209. (in Chinese)

[77]
WANG Y L, LI X, CAO Y, et al. Effect of the ACAA1 gene on preadipocyte differentiation in sheep[J]. Frontiers in Genetics, 2021, 12:649140.

DOI

[78]
ROGERS G R, MARKOVA N G, DE LAURENZI V, et al. Genomic organization and expression of the human fatty aldehyde dehydrogenase gene (FALDH)[J]. Genomics, 1997, 39(2):127-135.

DOI PMID

[79]
SMITH S, WITKOWSKI A, JOSHI A K. Structural and functional organization of the animal fatty acid synthase[J]. Progress in Lipid Research, 2003, 42(4):289-317.

DOI PMID

[80]
LIU G M, ZHANG Y M. Targeting FBPase is an emerging novel approach for cancer therapy[J]. Cancer Cell International, 2018, 18:36.

DOI

[81]
古再丽阿依·艾萨, 热衣兰木·包尔汉, 米热古丽·买买提, 等. FBP1基因突变导致FBPase缺乏症1例[J]. 中国医学工程, 2023, 31(4):130-132.

GUZAILIAYI A S, REYILANMU B E H, MIREGULI M M T, et al. One case of FBPase deficiency caused by FBP1 gene mutation[J]. China Medical Engineering, 2023, 31(4):130-132. (in Chinese)

[82]
陈灰, 李松建, 杜蕊, 等. 奶牛亚临床酮病血液生化指标特征分析及糖皮质激素影响肝细胞糖异生作用分子机制的研究[J/OL]. 中国预防兽医学报, 2023:1-10.(2023-05-24) [2023-10-01]. http://kns.cnki.net/kcms/detail/23.1417.s.20230523.1123.003.html

CHEN H, LI S J, DU R, et al. Analysis of blood biochemical parameters of subclinical ketosis and glucocorticoid-stimulated hepatocyte gluconeogenesis in diary cattle study on the molecular mechanism[J/OL]. Chinese Journal of Preventive Veterinary 2023:1-10.(2023-05-24) [2023-10-01]. http://kns.cnki.net/kcms/detail/23.1417.s.20230523.1123.003.htmlin Chinese)

[83]
ISPADA J, DA FONSECA JUNIOR A M, DE LIMA C B, et al. Tricarboxylic acid cycle metabolites as mediators of DNA methylation reprogramming in bovine preimplantation embryos[J]. International Journal of Molecular Sciences, 2020, 21(18):6868.

DOI

[84]
毛玉帅, 段亚冰, 周明国. 琥珀酸脱氢酶抑制剂类杀菌剂抗性研究进展[J]. 农药学学报, 2022, 24(5):937-948.

MAO Y S, DUAN Y B, ZHOU M G. Research progress of the resistance to succinate dehydrogenase inhibitors[J]. Chinese Journal of Pesticide Science, 2022, 24(5):937-948. (in Chinese)

[85]
林美佳, 曾也婷, 王心睿, 等. 异柠檬酸脱氢酶基因突变治疗的研究进展[J]. 协和医学杂志, 2023, 14(2):346-352.

LIN M J, ZENG Y T, WANG X R, et al. Research progress of isocitrate dehydrogenase gene mutation therapy[J]. Medical Journal of Peking Union Medical College Hospital, 2023, 14(2):346-352. (in Chinese)

[86]
YANKOVSKAYA V, HORSEFIELD R, TÖRNROTH S, et al. Architecture of succinate dehydrogenase and reactive oxygen species generation[J]. Science, 2003, 299(5607):700-704.

DOI PMID

Outlines

/