RESEARCH PAPER

Effects of Supplementation of Bacillus subtilis and β-Glucan in Cottonseed Protein Concentrate Diets on Growth Performance, Serum Biochemical Indices and Organismal Health of Juvenile Rainbow Trout (Oncorhynchus mykiss)

  • SHI Honghe , 1, 2 ,
  • LIU Yang 2 ,
  • WANG Di 2 ,
  • LU Shaoxia 2 ,
  • HAN Shicheng 2 ,
  • QIU Guangwen 1, 2 ,
  • WANG Chang’an 2 ,
  • ZHANG Hui , 1, * ,
  • LIU Hongbai , 2, *
Expand
  • 1 Animal Science and Technology College, Northeast Agricultural University, Harbin 150030, China
  • 2 Heilongjiang River Fisheries Research Institute, Chinese Academy of Fishery Sciences, Harbin 150070, China
*associate professor, E-mail: ;
professor, E-mail:

Received date: 2023-11-20

  Online published: 2024-06-07

Abstract

This experiment was conducted to investigate the effects of supplementation of Bacillus subtilis and β-glucan in cottonseed protein concentrate diets on growth performance, serum biochemical indices and organismal health of juvenile rainbow trout (Oncorhynchus mykiss). A total of 420 healthy juvenile rainbow trout with similar body weight of (21.66±0.08) g were randomly divided into 7 groups with 3 replicates per group and 20 trout per replicate. The control group (CON group) was fed the basal diet, the cottonseed protein concentrate group (CPC group) was fed the diet with 30% cottonseed protein concentrate equal to replace the fish meal in the basal diet, and the experimental groups were supplemented with 1×10⁶ CFU/g Bacillus subtilis (group Ⅰ), 1×10⁸ CFU/g Bacillus subtilis (group Ⅱ), 1×10⁸ CFU/g Bacillus subtilis lyophilized powder (group Ⅲ) and 0.1% (group Ⅳ) and 1.0% β-glucan (group Ⅴ) in the diets of CPC group, respectively. The experiment lasted for 8 weeks. The results showed as follows: 1) compared with CON group, the final body weight, weight gain rate (WGR) and specific growth rate (SGR) of juvenile rainbow trout in CPC group and experimental groups were significantly decreased (P<0.05), while the feed coefficient (FCR) was significantly increased (P<0.05); compared with CPC group, there were no significant differences in growth performance indices in experimental groups (P>0.05). 2) Compared with CON group, the serum glutamic-pyruvic transaminase (ALT) activity in CPC group was significantly increased (P<0.05); compared with CPC group, the serum ALT activity in experimental groups was significantly decreased except group Ⅲ (P<0.05); the serum lysozyme (LSZ) activity in experimental groups was significantly higher than that in CON and CPC groups (P<0.05). 3) Compared with CON group, the intestinal lipase and α-amylase activities of juvenile rainbow trout in CPC group were significantly decreased (P<0.05); compared with CPC group, the intestinal lipase activity in experimental groups was significantly increased (P<0.05), and the intestinal α-amylase activity in groups Ⅰ and Ⅱ was significantly increased (P<0.05). 4) Compared with CON group, the intestinal total antioxidant capacity (T-AOC) and catalase (CAT) activity of juvenile rainbow trout in CPC group were significantly decreased (P<0.05), while the intestinal malondialdehyde (MDA) content was significantly increased (P<0.05); compared with CPC group, the intestinal T-AOC and CAT activity in experimental groups were significantly increased (P<0.05), and the intestinal MDA content in groups Ⅱ, Ⅲ and Ⅴ was significantly decreased (P<0.05). 5) Compared with CON group, the mRNA relative expression levels of intestinal interleukin-1β (IL-1β), interleukin-8 (IL-8) and tumor necrosis factor-α (TNF-α) of juvenile rainbow trout in CPC group were significantly increased (P<0.05), while the mRNA relative expression levels of intestinal transforming growth factor-β (TGF-β) and interleukin-10 (IL-10) were significantly decreased (P<0.05); compared with CPC group, the mRNA relative expression levels of intestinal IL-1β, IL-8 and TNF-α mRNA in experimental groups were significantly decreased (P<0.05), the intestinal TGF-β mRNA relative expression level in experimental groups was significantly increased except group Ⅳ (P<0.05), and the intestinal IL-10 mRNA relative expression level in groups Ⅱ and Ⅴ was significantly increased (P<0.05). 6) Compared with CON group, the mRNA relative expression levels of intestinal claudin-1 (CLD1), occludin (OCLN), tricellulin (TRIC) and zonula occludens-1 (ZO-1) as well as complement 3 (C3) and complement 4 (C4) of juvenile rainbow trout in CPC group were significantly decreased (P<0.05); compared with CPC group, the mRNA relative expression levels of intestinal OCLN, TRIC, ZO-1, C3 and C4 in experimental groups were significantly increased except group Ⅳ (P<0.05). 7) Compared with CON group, the intestinal villus height of juvenile rainbow trout in CPC group was significantly decreased (P<0.05); compared with CPC group, the intestinal villus height in groups Ⅰ to Ⅲ was significantly increased (P<0.05), and the intestinal muscular thickness in group Ⅱ was significantly increased (P<0.05). 8) Compared with CON group, the Aeromonas salmonicida number in liver and spleen of juvenile rainbow trout in CPC group was significantly increased (P<0.05); compared with CPC group, except group Ⅳ, Aeromonas salmonicida number in liver in experimental groups was significantly decreased (P<0.05), and Aeromonas salmonicida number in spleen in experimental groups was significantly decreased (P<0.05). In conclusion, the supplementation of Bacillus subtilis and β-glucan in cottonseed protein concentrate diets has no significant effects on the growth performance of juvenile rainbow trout, but can improve the serum biochemical indices, intestinal health and the ability to resist Aeromonas salmonicida. In addition, the spray process of adding 1×10⁸ CFU/g Bacillus subtilis and adding 1.0% β-glucan have better effects on juvenile rainbow trout.

Cite this article

SHI Honghe , LIU Yang , WANG Di , LU Shaoxia , HAN Shicheng , QIU Guangwen , WANG Chang’an , ZHANG Hui , LIU Hongbai . Effects of Supplementation of Bacillus subtilis and β-Glucan in Cottonseed Protein Concentrate Diets on Growth Performance, Serum Biochemical Indices and Organismal Health of Juvenile Rainbow Trout (Oncorhynchus mykiss)[J]. Chinese Journal of Animal Nutrition, 2024 , 36(6) : 3857 -3875 . DOI: 10.12418/CJAN2024.331

鱼粉是肉食性鱼类的重要蛋白质来源,但由于水产养殖业需求的不断增长且鱼粉产量相对稳定,致使鱼粉的价格持续高涨[1]。长期以来,寻找更稳定、更具成本效益和可持续的蛋白质原料替代鱼粉一直是水产动物营养饲料研究中的重点领域[2]。以大豆为代表的植物性蛋白源由于来源广泛、成本较为低廉且具有较好的饲料鱼粉替代效果,在饲料产业上已有较为广泛地应用[3-4]。但大豆为粮食类原料,且我国大豆进口依存度较高,因此寻找优质的非粮植物性蛋白质源显得尤为重要。我国是世界第一产棉大国,棉籽资源丰富,年产量约800万t,其中新疆是主要棉籽产区,产量达到700万t左右[5]。通过棉籽加工制成的棉籽浓缩蛋白具有蛋白质含量高、氨基酸组成较为均衡以及抗营养因子含量低等优点[6-7],得到了学界和产业界的高度重视[5,8]。研究表明,棉籽浓缩蛋白可以部分替代肉食性鱼类饲料鱼粉,但不同种类棉籽浓缩蛋白的适应性存在一定的差异[9-10],且高比例替代会对肉食性鱼类的生长性能、代谢功能以及肠道健康造成严重负面作用[11]
通过在饲料中添加功能性添加剂改善水产养殖动物的生长性能和健康水平已被证明是一种行之有效的方法。其中,以枯草芽孢杆菌(Bacillus subtilis)为代表的益生菌以及β-葡聚糖的正面作用均被证实。枯草芽孢杆菌是最常用、最具特色的一类芽孢杆菌,在水产养殖上的应用研究也比较多,该菌对养殖动物和人无病原性、毒性及毒副作用,且易于生产和保存[12]。已经有许多研究表明,在肉食性鱼类饲料中添加枯草芽孢杆菌可以改善其生长性能、免疫功能和抗氧化能力等,且在虹鳟(Oncorhynchus mykiss)[13-15]、大口黑鲈(Micropterus salmoides)[16]及珍珠龙胆石斑鱼(Epinephelus fuscoguttatus♀×E. lanceolatus♂)[17]中均有证实。β-葡聚糖是一种以纤维形式存在的均一多糖,广泛存在于谷物(如大麦、燕麦、小麦等)和微生物(如酵母、细菌、真菌等)的细胞壁中,是构成生物细胞壁的主要材料,且具有多种生物学结构与活性[18-19]。许多研究表明,在肉食性鱼类饲料中添加β-葡聚糖可以改善其生长性能、免疫功能、抗氧化能力及抗病力等[20-24]
虹鳟属于鲑科太平洋鲑属,是一种典型的肉食性冷水性鱼类,对饲料蛋白质的需求很高,一般需要40%以上的蛋白质,且优质鱼粉仍然是商业鳟鱼饲料的主要蛋白质来源之一[25]。本团队前期研究结果显示,饲料中使用超过75%的棉籽浓缩蛋白替代鱼粉会影响虹鳟的生长和血液代谢指标,并损害肠道健康[11]。因此,本文通过在棉籽浓缩蛋白基础饲料中添加不同水平的枯草芽孢杆菌和β-葡聚糖,研究二者对高比例棉籽浓缩蛋白饲喂虹鳟幼鱼生长性能、血清生化指标和机体健康的影响,探讨棉籽浓缩蛋白营养的改进策略,以期为优化肉食性鱼类饲料配方提供参考。

1 材料与方法

1.1 试验材料

试验所用棉籽浓缩蛋白含有65%粗蛋白质,其中游离棉酚含量为230 mg/kg;枯草芽孢杆菌由中国水产科学研究院黑龙江水产研究所水产病害与防治实验室提供[26];β-葡聚糖产品为市售,其中β-葡聚糖含量>70%。

1.2 试验设计

驯化21 d后,试验选择体质量[(21.66±0.08) g]基本一致的健康虹鳟幼鱼420尾,随机分为7组,每组3个重复,每个重复20尾。对照组(CON组)饲喂基础饲料,棉籽浓缩蛋白组(CPC组)饲喂用30%棉籽浓缩蛋白等量替代基础饲料中鱼粉的饲料,试验组分别在CPC组饲料的基础上添加1×10⁶ CFU/g枯草芽孢杆菌(Ⅰ组)、1×108 CFU/g枯草芽孢杆菌(Ⅱ组)、1×108 CFU/g枯草芽孢杆菌冻干粉(Ⅲ组)以及在CPC组饲料基础上添加0.1%(Ⅳ组)和1.0% β-葡聚糖(Ⅴ组)。试验期8周。

1.3 试验饲料

本试验配制了7种等氮(粗蛋白质含量47%)和等脂(粗脂肪含量17%)饲料,其组成及营养水平见表1。所有固体原料经前处理(粉碎后过60目筛)后,采用逐级扩大法预混合,然后采用实验室制粒机(HKJ-218,无锡同力粮机有限公司)加工成直径为1.5 mm的颗粒。所有饲料分别在通风烘箱(60 ℃,1.5 h)中烘干后,在4 ℃冰箱中保存待用。Ⅰ组和Ⅱ组的枯草芽孢杆菌待饲料烘干后平铺,均匀喷洒并自然风干;Ⅲ组的枯草芽孢杆菌冻干粉直接混入饲料中制粒。
表1 试验饲料组成及营养水平(干物质基础)

Table 1 Composition and nutrient levels of experimental diets (DM basis)%

项目
Items
组别 Groups
CON CPC
原料 Ingredients
鱼粉 Fish meal 30.00
黑水虻虫粉 Black soldier fly meal 5.00 5.00 5.00 5.00 5.00 5.00 5.00
棉籽浓缩蛋白 Cottonseed protein concentrate 30.00 30.00 30.00 30.00 30.00 30.00
玉米蛋白粉 Corn gluten meal 12.00 12.00 12.00 12.00 12.00 12.00 12.00
大豆浓缩蛋白 Soy protein concentrate 15.00 15.00 15.00 15.00 15.00 15.00 15.00
谷朊粉 Wheat gluten meal 2.00 2.00 2.00 2.00 2.00 2.00 2.00
面粉 Wheat flour 19.58 18.83 18.83 18.83 18.83 18.73 17.83
鱼油 Fish oil 12.00 12.00 12.00 12.00 12.00 12.00 12.00
预混料 Premix1) 1.00 1.00 1.00 1.00 1.00 1.00 1.00
L-赖氨酸 L-lysine (98%) 1.00 1.75 1.75 1.75 1.75 1.75 1.75
DL-蛋氨酸 DL-methionine (99%) 0.30 0.30 0.30 0.30 0.30 0.30 0.30
牛磺酸 Taurine (99%) 0.50 0.50 0.50 0.50 0.50 0.50 0.50
海藻酸钠 Sodium alginate 1.00 1.00 1.00 1.00 1.00 1.00 1.00
胆碱 Choline (50%) 0.60 0.60 0.60 0.60 0.60 0.60 0.60
二丁基羟基甲苯 BHT (>99.0%) 0.02 0.02 0.02 0.02 0.02 0.02 0.02
β-葡聚糖 β-glucan 0.10 1.00
合计 Total 100.00 100.00 100.00 100.00 100.00 100.00 100.00
营养水平 Nutrient levels2)
粗蛋白质 Crude protein 47.40 47.58 47.31 47.20 47.67 47.31 47.36
粗脂肪 Crude lipid 17.14 16.89 16.79 17.03 17.05 16.95 17.25
粗灰分 Ash 5.60 5.64 5.59 5.60 5.58 5.58 5.59

1)每千克预混料含有 One kilogram of premix contained the following:VA 750 000 IU,VD3 200 000 IU,VE 6 000 mg,VK3 2 000 mg,VB1 1 200 mg,VB2 1 200 mg,VB6 1 200 mg,VB12 8 mg,VC 21 000 mg,D-泛酸钙 D-calcium pantothenate 2 000 mg,烟酰胺 niacinamide 9 000 mg,叶酸 folic acid 370 mg,D-生物素 D-biotin 15 mg,肌醇 inositol 10 000 mg,MgSO4 6 000 mg,ZnSO4 4 000 mg,MnSO4 2 500 mg,CuSO4 2 500 mg,FeSO4 2 500 mg,CoSO4 160 mg,Ca(IO3)2 200 mg,Na2SeO3 40 mg。

2)营养水平为实测值。Nutrient levels were measured values.

1.4 饲养管理

养殖试验在中国水产科学研究院黑龙江水产研究所循环水养殖第1车间进行,总水体容积为8 m3。试验期间,每天于08:30和15:30各人工饱饲投喂1次。养殖水体水流速度保持在0.4 m/s,水温控制在12.5~13.5 ℃,光周期为12 h白天∶12 h黑暗,每天换水量为总水体容量的15%~20%,溶解氧浓度保持在8 mg/L以上。

1.5 样品采集

试验结束时,试验鱼经麻醉(MS-222,200 mg/L)后测量体长并称重。每重复随机选取3尾鱼,用于全鱼常规营养成分含量的测定。每重复随机选取7尾鱼,采集血液、肝脏、脾脏和全肠,其中4尾鱼通过尾静脉采集血液,并在4 ℃下以955×g离心10 min后,收集上清液作为血清并保存在-80 ℃冰箱中;肝脏、脾脏和全肠采集完成后保存在液氮中,用于后续检测;另取3尾鱼的中肠,去除肠道内容物,并将其放在甲醛溶液中固定,用于进行肠道组织形态观察。

1.6 测定指标及方法

1.6.1 生长性能测定

生长性能指标计算公式如下:

增重率(weight gain rate,WGR)=100×(Wt-W0)/W0;

特定生长率(specific growth rate,SGR)=100×(lnWt-lnW0)/t;

饲料系数(feed coefficient,FCR)=Wf/(Wt-W0);

肥满度(condition factor,CF)=100×Wt/ L t 3;

脏体比(viscerosomatic index,VSI)=100×Wv/Wt;

肝体比(hepatosomatic index,HSI)=100%×Wh/Wt

式中:W0为鱼初始体质量(g);Wt为鱼终末体质量(g);Lt为鱼终末体长(cm);Wf为饲料摄入量(g);Wv为鱼内脏团质量(g);Wh为鱼肝脏质量(g);t为试验天数(d)。

1.6.2 常规营养成分含量测定

采用烘干法(GB/T 6435—2014),在(105±1) ℃烘箱中将样品烘干至恒重,测定饲料和全鱼样品中水分含量;采用杜马斯燃烧法(GB/T 24318—2009)测定粗蛋白质含量;采用索氏抽提法(GB/T 6433—2006),以乙醚为抽提剂测定粗脂肪含量;采用灼烧法(GB/T 6438—2007),在马弗炉(550 ℃)中充分灼烧测定粗灰分含量。

1.6.3 血清生化指标和肠道消化酶活性测定

采用全自动生化分析仪(BECKMAN CX4)通过标准分光光度法测定血清生化指标,采用试剂盒(南京建成生物工程研究所)测定肠道消化酶活性。

1.6.4 肠道组织形态

将甲醛溶液中固定的中肠取出,流水冲洗数次后利用梯度浓度乙醇脱水,最后将肠道组织包埋于石蜡中;包埋后的蜡块采用切片机(HistoCore MULTICUT,Leica)切成4 μm厚的切片;切片经过乙醇脱色、苏木精-伊红染色以及中性树脂密封后保存,在显微镜(MD 4000B,Leica)下检查肠道组织形态,并测量绒毛高度、绒毛宽度和肌层厚度。

1.6.5 肠道抗氧化指标测定

将采集的肠道样品从液氮中取出,在研钵中研磨成粉,加入9倍肠道样品重量的预冷生理盐水,置于匀浆机(Scientz-48L,宁波新芝生物科技股份有限公司)中,制成10%组织匀浆,然后在低温高速离心机(H2050R,湖南湘仪实验室仪器开发有限公司)上在4 ℃、1 698×g下离心10 min,取上清液,将上清液置于1.5 mL离心管中,稀释后保存于-80 ℃冰箱中,用于后续测定。
采用试剂盒(南京建成生物工程研究所)测定肠道总抗氧化能力(total antioxidant capacity,T-AOC)和过氧化氢酶(catalase,CAT)、超氧化物歧化酶(superoxide dismutase,SOD)、谷胱甘肽过氧化物酶(glutathione peroxidase,GSH-Px)活性以及丙二醛(malondialdehyde,MDA)含量。

1.6.6 肠道免疫因子和紧密连接蛋白基因表达测定

将肠道样品通过液氮冷冻研磨的方式研磨成粉,采用TRIzol(RNAiso Plus,Code No. 9109,TaKaRa)提取肠道总RNA,然后进行反转录以合成cDNA。然后在Applied Biosystems 7500 PCR系统中使用TaKaRa TB Green Premix Ex Taq Ⅱ (Tli RNaseH Plus)试剂盒进行实时荧光定量PCR。本研究中使用的引物的有效性采用已公布的技术[27]进行评估,具体引物序列见表2。以β-肌动蛋白(β-actin)为内参基因,采用采用2-ΔΔCt[28]计算目的基因的mRNA相对表达量。
表2 实时荧光定量PCR引物序列

Table 2 Primer sequences for RT-qPCR

目的基因
Target genes
引物序列
Primer sequences (5'—3')
登录号
Accession number
β-肌动蛋白 β-actin F:ACAGACTGTACCCATCCCAAAC
R:AAAAAGCGCCAAAATAACAGAA
AJ438158
补体3 C3 F:GGCCAGTCCCTGGTGGTTA
R:GGTGGACTGTGTGGATCCGTA
L24433
补体4 C4 F:TCTACAACCCTACACAGCAAGTGAG
R:TGCCCGCAGCATTAAAAATAG
AJ544262
白细胞介素-1β IL-1β F:ACCGAGTTCAAGGACAAGGA
R:CATTCATCAGGACCCAGCAC
AJ223954
白细胞介素-8 IL-8 F:CACAGACAGAGAAGGAAGGAAAG
R:TGCTCATCTTGGGGTTACAGA
AJ279069
肿瘤坏死因子-α TNF-α F:GGGGACAAACTGTGGACTGA
R:GAAGTTCTTGCCCTGCTCTG
AJ277604
白细胞介素-10 IL-10 F:CGACTTTAAATCTCCCATCGAC
R:GCATTGGACGATCTCTTTCTTC
AB118099
转化生长因子-β TGF-β F:AGATAAATCGGAGAGTTGCTGTG
R:CCTGCTCCACCTTGTGTTGT
AJ007836
封闭蛋白-1 CLD1 F:GAGGACCAGGAGAAGAAGG
R:AGCCCCAACCTACGAAC
GQ476574
闭合蛋白 OCLN F:CAGCCCAGTTCCTCCAGTAG
R:GCTCATCCAGCTCTCTGTCC
KC603902
三细胞紧密连接蛋白 TRIC F:GTCACATCCCCAAACCAGTC
R:GTCCAGCTCGTCAAACTTCC
HQ656020
闭锁小带蛋白-1 ZO-1 F:AAGGAAGGTCTGGAGGAAGG
R:CAGCTTGCCGTTGTAGAGG
BK008768

1.6.7 细菌载量试验

试验结束后,每组每个重复随机挑选10尾鱼用MS222麻醉,采用8.8×10⁹ CFU/mL的杀鲑气单胞菌(Aeromonas salmonicida)HA01通过腹腔注射的方式进行人工感染,注射剂量为100 μL/尾。感染3 d后,取出试验鱼的肝脏和脾脏,将组织称重后放入1.5 mL离心管中,按照1∶10的比例在离心管中加入磷酸盐缓冲液(PBS),再加入组织研磨珠,使用高通量组织匀浆机(A5121104,宁波新芝生物科技股份有限公司)进行研磨,1 000 r/min振荡30 s,取20 μL的混浊液体滴在胰酪大豆胨琼脂(TSA)培养基上,使用涂布棒推铺均匀,在37℃下培养24 h后,通过单菌落计数的方式计算各组织中杀鲑气单胞菌的数量。

1.7 数据统计与分析

试验数据采用SPSS 21.0软件进行单因素方差分析(one-way ANOVA)和Duncan氏法多重比较,结果数据以“平均值±标准差(mean±SD)”形式表示,P<0.05表示差异显著;采用GraphPad Prism 9.0软件进行绘图。

2 结果与分析

2.1 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼生长性能的影响

表3可知,与CON组相比,CPC组和各试验组虹鳟幼鱼终末体质量、WGR和SGR均显著降低(P<0.05),FCR均显著提高(P<0.05);与CPC组相比,各试验组生长性能指标均无显著差异(P>0.05);各组间VSI和HSI均无显著差异(P>0.05)。
表3 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼生长性能的影响

Table 3 Effects of Bacillus subtilis and β-glucan on growth performance of juvenile rainbow trout (Oncorhynchus mykiss)

项目
Items
组别 Groups
CON CPC
初始体质量
IBW/g
21.75
±0.09
21.89
±0.06
21.41
±0.44
21.81
±0.03
21.44
±0.16
21.68
±0.08
21.67
±0.11
终末体质量
FBW/g
98.20
±4.49b
79.37
±0.60a
77.77
±2.64a
83.27
±2.16a
77.22
±0.99a
75.69
±0.89a
76.12
±1.58a
增重率 WGR/% 351.76
±22.38b
262.64
±3.43a
263.17
±7.54a
281.81
±9.80a
260.11
±3.64a
249.17
±4.71a
251.30
±8.73a
特定生长率
SGR/(%/d)
2.69
±0.09c
2.30
±0.02ab
2.30
±0.04ab
2.39
±0.05b
2.29
±0.02ab
2.23
±0.02a
2.24
±0.04ab
饲料系数
FCR
0.91
±0.02a
1.01
±0.01b
1.00
±0.01b
1.01
±0.02b
1.01
±0.01b
1.01
±0.01b
1.02
±0.01b
肥满度
CF/(g/cm3)
1.37
±0.02ab
1.34
±0.02ab
1.39
±0.02b
1.38
±0.02b
1.40
±0.02b
1.40
±0.02b
1.31
±0.02a
脏体比
VSI/%
13.55
±0.64
13.65
±0.44
13.68
±0.39
13.14
±0.50
14.56
±0.32
13.51
±0.69
14.43
±0.69
肝体比
HSI/%
1.43
±0.09
1.33
±0.05
1.34
±0.05
1.40
±0.07
1.38
±0.06
1.36
±0.06
1.41
±0.06

同行数据肩标无字母或相同字母表示差异不显著(P>0.05),不同字母表示差异显著(P<0.05)。下表同。

In the same row, values with no letter or the same letter superscripts mean no significant difference (P>0.05), while with different letter superscripts mean significant difference (P<0.05). The same as below.

2.2 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼全鱼常规营养成分含量的影响

表4可知,与CON组相比,Ⅱ组和Ⅴ组虹鳟幼鱼全鱼水分含量显著提高(P<0.05);与CPC组相比,各试验组全鱼水分含量无显著差异(P>0.05)。与CON组和CPC组相比,Ⅳ组和Ⅴ组全鱼粗脂肪含量显著降低(P<0.05),且Ⅴ组显著低于Ⅳ组(P<0.05);Ⅰ组~Ⅲ组全鱼粗脂肪含量无显著差异(P>0.05)。与CON组相比,CPC组和各试验组全鱼粗灰分含量均显著提高(P>0.05),且CPC组和各试验组间无显著差异(P>0.05)。各组间全鱼粗蛋白质含量无显著差异(P>0.05)。
表4 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼全鱼常规营养成分含量的影响

Table 4 Effects of Bacillus subtilis and β-glucan on conventional nutrient contents in whole body of juvenile rainbow trout (Oncorhynchus mykiss)%

项目
Items
组别 Groups
CON CPC
水分 Moisture 67.05
±1.73a
68.11
±0.68ab
68.57
±1.21ab
71.31
±1.05b
70.03
±0.65ab
69.33
±0.83ab
71.40
±0.57b
粗蛋白质 Crude protein 57.17
±0.25
56.76
±0.24
56.79
±0.29
57.13
±0.30
57.04
±0.16
56.91
±0.34
57.01
±0.14
粗脂肪 Crude lipid 39.02
±0.76c
38.60
±0.44c
38.53
±0.51c
39.63
±0.71c
37.88
±0.78bc
36.29
±0.36b
34.23
±0.99a
粗灰分 Ash 7.37
±0.03a
9.18
±0.04b
9.10
±0.03b
9.15
±0.03b
9.10
±0.04b
9.15
±0.04b
9.09
±0.03b

2.3 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼血清生化指标的影响

表5可知,与CON组相比,CPC组和各试验组虹鳟幼鱼血清白蛋白(ALB)含量均无显著差异(P>0.05),但Ⅱ组血清ALB含量显著高于CPC组(P<0.05);CPC组和各试验组血清碱性磷酸酶(ALP)活性显著降低(P<0.05),且CPC组和各试验组间无显著差异(P>0.05);CPC组血清谷丙转氨酶(ALT)活性显著提高(P<0.05),各试验组血清ALT活性无显著差异(P>0.05),且除Ⅲ组外,其他试验组血清ALT活性均显著低于CPC组(P<0.05);CPC组和各试验组血清高密度脂蛋白胆固醇(HDL-C)和低密度脂蛋白胆固醇(LDL-C)含量均显著降低(P<0.05),且各试验组血清HDL-C和LDL-C含量与CPC组相比均无显著差异(P>0.05);CPC组血清总胆汁酸(TBA)含量显著提高(P<0.05),各试验组血清TBA含量均无显著差异(P>0.05),且与CPC组相比亦无显著差异(P>0.05);CPC组和各试验组血清总胆固醇(TC)含量显著降低(P<0.05),且CPC组和各试验组间无显著差异(P>0.05);CPC组血清甘油三酯(TG)含量显著提高(P<0.05),各试验组血清TG含量无显著差异(P>0.05),且均显著低于CPC组(P<0.05);各试验组血清溶菌酶(LSZ)活性均显著高于CON组和CPC组(P<0.05)。
表5 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼血清生化指标的影响

Table 5 Effects of Bacillus subtilis and β-glucan on serum biochemical indices of juvenile rainbow trout (Oncorhynchus mykiss)

项目
Items
组别 Groups
CON CPC
白蛋白
ALB/(g/L)
18.67
±0.49ab
17.63
±0.94a
18.65
±0.58ab
20.23
±0.40b
17.83
±0.80a
18.22
±0.56ab
18.57
±0.68ab
碱性磷酸酶
ALP/(U/L)
498.07
±49.42b
253.78
±25.14a
264.55
±12.83a
282.40
±33.52a
217.38
±10.60a
281.15
±20.41a
288.40
±12.68a
谷丙转氨酶
ALT/(U/L)
14.87
±1.31a
21.75
±2.48b
16.33
±1.30a
15.90
±0.86a
17.78
±0.90ab
16.72
±1.23a
16.00
±0.97a
高密度脂蛋白胆固醇
HDL-C/(mmol/L)
4.04
±0.15c
2.91
±0.19ab
3.13
±0.11b
3.10
±0.10b
2.57
±0.06a
2.99
±0.15ab
2.94
±0.18ab
低密度脂蛋白胆固醇
LDL-C/(mmol/L)
1.56
±0.09b
1.33
±0.12a
1.16
±0.06a
1.15
±0.04a
1.10
±0.04a
1.10
±0.08a
1.12
±0.06a
总胆汁酸
TBA/(μmmol/L)
2.35
±0.79a
5.78
±0.88b
3.87
±0.66ab
3.67
±1.14ab
3.58
±0.76ab
4.40
±0.96ab
3.67
±0.80ab
总胆固醇
TC/(mmol/L)
11.77
±0.52b
8.44
±0.67a
8.17
±0.22a
8.37
±0.27a
7.79
±0.30a
7.95
±0.53a
7.70
±0.27a
甘油三酯
TG/(mmol/L)
6.77
±0.49a
8.67
±0.65b
6.10
±0.36a
6.91
±0.54a
6.21
±0.45a
6.35
±0.70a
6.80
±0.38a
溶菌酶
LSZ/(U/mL)
14.48
±1.65a
24.25
±3.45a
58.11
±10.12b
44.38
±4.94b
56.70
±5.34b
60.54
±4.65b
51.25
±4.99b

2.4 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道消化酶活性的影响

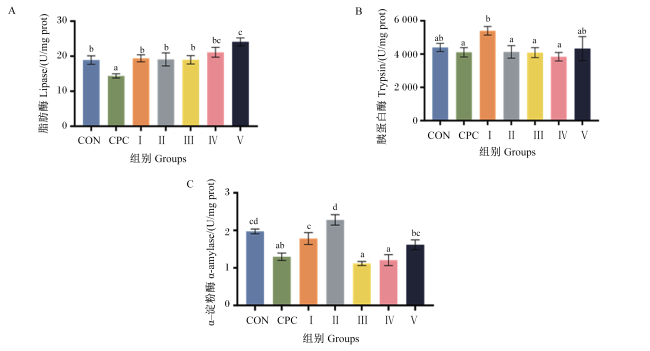
图1-A所示,与CON组相比,CPC组虹鳟幼鱼肠道脂肪酶活性显著降低(P<0.05),Ⅴ组肠道脂肪酶活性显著提高(P<0.05),且各试验组肠道脂肪酶活性均显著高于CPC组(P<0.05);此外,Ⅴ组肠道脂肪酶活性还显著高于Ⅰ组~Ⅲ组(P<0.05)。如图1-B所示,与CON组相比,CPC组和各试验组肠道胰蛋白酶活性均无显著差异(P>0.05),但Ⅰ组肠道胰蛋白酶活性显著高于CPC组和Ⅱ组~Ⅳ组(P<0.05)。如图1-C所示,与CON组相比,CPC组、Ⅲ组和Ⅳ组肠道α-淀粉酶活性显著降低(P<0.05),其他各组肠道α-淀粉酶活性无显著差异(P>0.05);与CPC组相比,Ⅰ组和Ⅱ组肠道α-淀粉酶活性显著提高(P<0.05),且显著高于Ⅲ组和Ⅳ组(P<0.05),并且Ⅱ组肠道α-淀粉酶活性显著高于Ⅴ组(P<0.05)。
图1 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道消化酶活性的影响

数据柱标记不同字母表示差异显著(P<0.05)。下图同。

Fig.1 Effects of Bacillus subtilis and β-glucan on intestinal digestive enzyme activities of juvenile rainbow trout (Oncorhynchus mykiss)

Value columns with different letters mean significant difference (P<0.05). The same as below.

2.5 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道抗氧化指标的影响

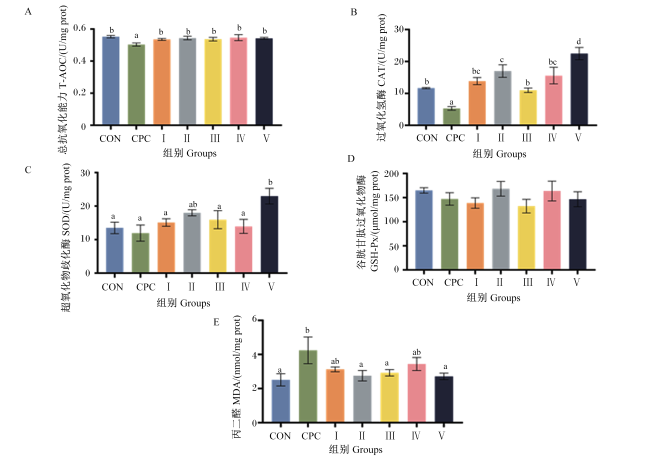
图2所示,与CON组相比,CPC组虹鳟幼鱼肠道T-AOC和CAT活性显著降低(P<0.05),肠道MDA含量显著提高(P<0.05);各试验组肠道T-AOC无显著差异(P>0.05),且均显著高于CPC组(P<0.05);Ⅱ组和Ⅴ组肠道CAT活性显著提高(P<0.05),且各试验组肠道CAT活性均显著高于CPC组(P<0.05);各试验组肠道MDA含量无显著差异(P>0.05),但Ⅱ组、Ⅲ组和Ⅴ组肠道MDA含量显著低于CPC组(P<0.05)。与CON组和CPC组相比,Ⅴ组肠道SOD活性显著提高(P<0.05),其他试验组肠道SOD活性无显著差异(P>0.05)。各组间肠道GSH-Px活性均无显著差异(P>0.05)。
图2 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道抗氧化指标的影响

Fig.2 Effects of Bacillus subtilis and β-glucan on intestinal antioxidant indices of juvenile rainbow trout (Oncorhynchus mykiss)

2.6 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道免疫因子和紧密连接蛋白基因表达的影响
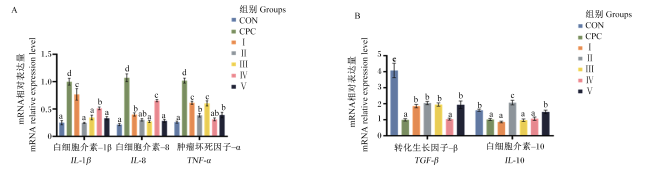
图3所示,与CON组相比,CPC组虹鳟幼鱼肠道白细胞介素-1β(IL-1β)、白细胞介素-8(IL-8)和肿瘤坏死因子-α(TNF-α)mRNA相对表达量显著提高(P<0.05);与CPC组相比,各试验组肠道IL-1βIL-8和TNF-α mRNA相对表达量均显著降低(P<0.05),且Ⅱ组、Ⅲ组和Ⅴ组肠道IL-1βIL-8 mRNA相对表达量与CON组相比无显著差异(P>0.05),Ⅳ组肠道TNF-αmRNA相对表达量与CON组相比无显著差异(P>0.05)。与CON组相比,CPC组虹鳟幼鱼肠道转化生长因子-β(TGF-β)和白细胞介素-10(IL-10)mRNA相对表达量显著降低(P<0.05);与CPC组相比,除Ⅳ组外,其他试验组肠道TGF-β mRNA相对表达量均显著提高(P<0.05),Ⅱ组和Ⅴ组肠道IL-10 mRNA相对表达量显著提高(P<0.05),且Ⅱ组肠道IL-10 mRNA相对表达量显著高于CON组(P<0.05)。
图3 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道炎性因子基因表达的影响

Fig.3 Effects of Bacillus subtilis and β-glucan on gene expression of intestinal inflammatory factors of juvenile rainbow trout (Oncorhynchus mykiss)

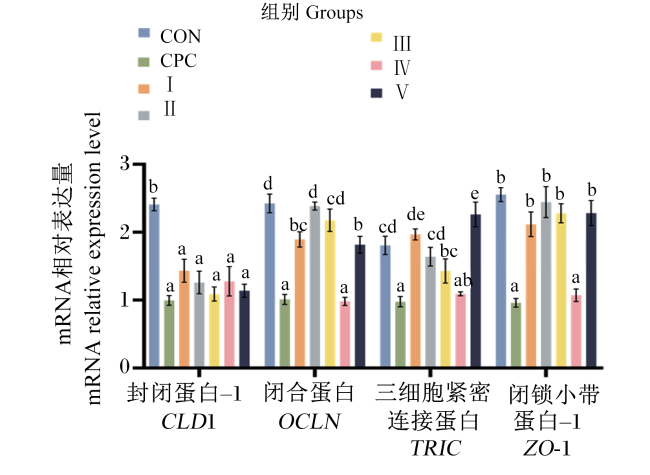
图4所示,与CON组相比,CPC组虹鳟幼鱼肠道封闭蛋白-1(CLD1)、闭合蛋白(OCLN)、三细胞紧密连接蛋白(TRIC)和闭锁小带蛋白-1(ZO-1)mRNA相对表达量均显著降低(P<0.05)。与CPC组相比,除Ⅳ组外,其他试验组肠道OCLNTRICZO-1 mRNA相对表达量均显著提高(P<0.05),且Ⅱ组和Ⅲ组肠道OCLNTRICZO-1 mRNA相对表达量与CON组相比无显著差异(P>0.05),Ⅴ组肠道TRIC mRNA相对表达量显著高于CON组(P<0.05)。
图4 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道紧密连接蛋白基因表达的影响

Fig.4 Effects of Bacillus subtilis and β-glucan on gene expression of intestinal tight junction proteins of juvenile rainbow trout (Oncorhynchus mykiss)

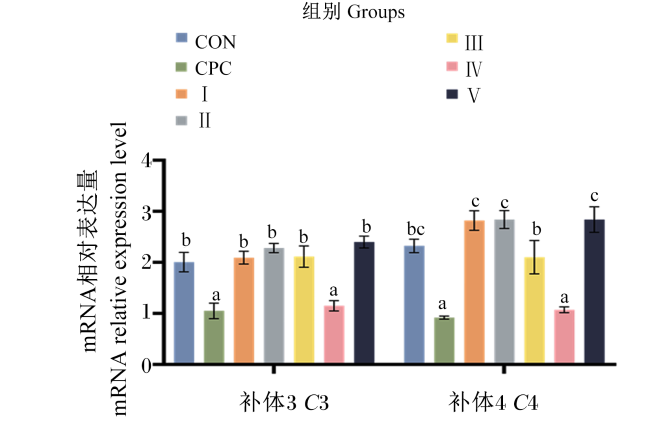
图5所示,与CON组相比,CPC组虹鳟幼鱼肠道补体3(C3)和补体4(C4)mRNA相对表达量均显著降低(P<0.05)。与CPC相比,除Ⅳ组外,其他试验组肠道C3和C4 mRNA相对表达量均显著提高(P<0.05),且与CON组相比均无显著差异(P>0.05)。
图5 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道补体基因表达的影响

Fig.5 Effects of Bacillus subtilis and β-glucan on gene expression of intestinal complement of juvenile rainbow trout (Oncorhynchus mykiss)

2.7 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道组织形态的影响

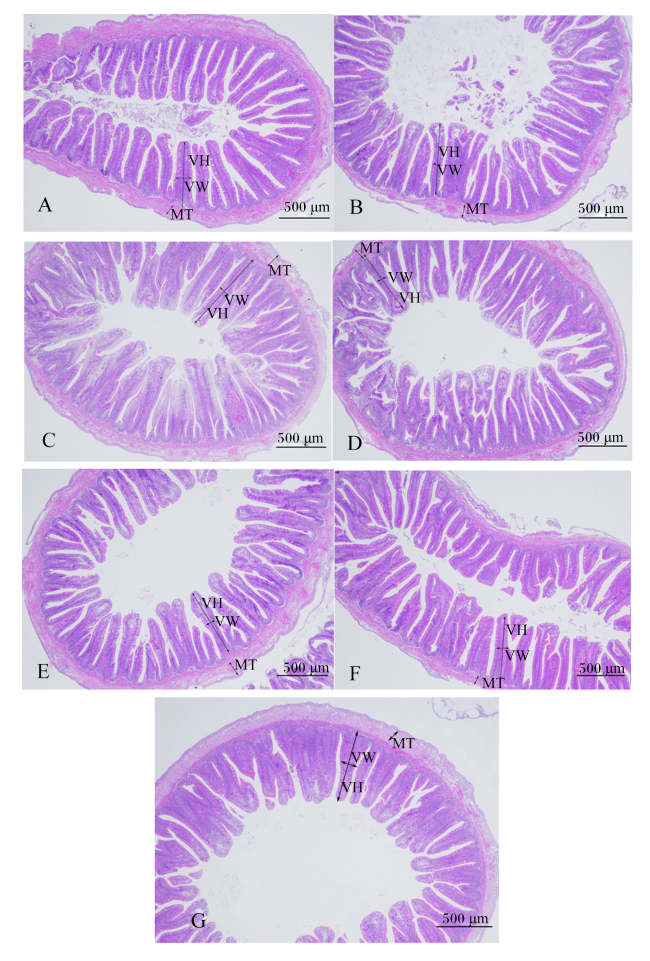
表6图6可知,与CON组相比,CPC组虹鳟幼鱼肠道绒毛高度显著降低(P<0.05);与CPC组相比,Ⅰ组~Ⅲ组肠道绒毛高度显著提高(P<0.05),且Ⅰ组和Ⅱ组肠道绒毛高度显著高于CON组(P<0.05)。与CON和CPC组相比,各试验组肠道绒毛宽度均无显著差异(P>0.05),但Ⅰ组和Ⅱ组肠道绒毛宽度显著高于Ⅳ组(P<0.05)。与CPC组相比,Ⅱ组肠道肌层厚度显著提高(P<0.05)。
表6 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道组织形态的影响

Table 6 Effects of Bacillus subtilis and β-glucan on intestinal tissue morphology of juvenile rainbow trout (Oncorhynchus mykiss)μm

项目
Items
组别 Groups
CON CPC
绒毛高度
Villus height
709.68
±13.00c
614.18
±23.11a
769.21
±27.32d
813.85
±9.61d
675.45
±8.88bc
634.33
±13.83ab
667.71
±22.37abc
绒毛宽度
Villus width
104.09
±5.26ab
99.76
±7.85ab
109.13
±3.43b
111.21
±4.37b
100.51
±12.01ab
94.10
±7.92a
106.02
±2.05ab
肌层厚度
Muscular thickness
123.47
±3.41bc
104.85
±12.80ab
124.08
±3.93bc
142.49
±2.79c
111.58
±11.53ab
96.41
±4.09a
105.43
±2.02ab
图6 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道组织形态的影响

VH:绒毛高度 villus height;VW:绒毛宽度 villus width;MT:肌层厚度 muscular thickness。

A~G分别表示CON组、CPC组、Ⅰ组、Ⅱ组、Ⅲ组、Ⅳ组和Ⅴ组。A to G represented CON group, CPC group, group Ⅰ, group Ⅱ, group Ⅲ, group Ⅳ and group Ⅴ, respectively.

Fig.6 Effects of Bacillus subtilis and β-glucan on intestinal tissue morphology of juvenile rainbow trout (Oncorhynchus mykiss)

2.8 细菌载量试验结果

表7可知,与CON组相比,CPC组虹鳟幼鱼肝脏和脾脏杀鲑气单胞菌数量显著提高(P<0.05),各试验组肝脏和脾脏杀鲑气单胞菌数量均无显著差异(P>0.05)。与CPC组相比,除Ⅳ组外,其他试验组肝脏鲑气单胞菌数量显著降低(P<0.05),各试验组脾脏杀鲑气单胞菌数量均显著降低(P<0.05)。
表7 枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼感染杀鲑气单胞菌后肝脏和脾脏细菌载量的影响

Table 7 Effects of Bacillus subtilis and β-glucan on bacterial load in liver and spleen of juvenile rainbow trout (Oncorhynchus mykiss) infected with Aeromonas salmonicidaCFU/g

项目
Items
组别 Groups
CON CPC
肝脏 Liver 5 638.42
±780.96ab
12 825.34
±4 346.66c
1 044.03
±142.04a
2 382.72
±213.84ab
3 405.65
±1 473.10ab
9 369.56
±3 561.13bc
1 122.08
±336.69a
脾脏 Spleen 19 520.56
±3 069.94a
53 670.39
±10 785.77b
14 189.55
±7 998.43a
7 490.03
±731.75a
17 219.40
±3 945.15a
12 220.18
±3 447.95a
5 404.59
±563.10a

3 讨论

3.1 棉籽浓缩蛋白饲料添加枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼生长性能的影响

研究表明,棉籽蛋白作为一种新型植物蛋白质源,可以部分替代肉食性鱼类饲料中的鱼粉而不会对其生长产生不良影响,在虹鳟[9]、大口黑鲈[7]及卵形鲳鲹(Trachinotus ovatus)[29]上的研究结果均证实了棉籽蛋白部分替代饲料中鱼粉的有效性。然而,高比例的棉籽蛋白替代饲料鱼粉会导致虹鳟[10-11]和大口黑鲈[30]等肉食性鱼类生长性能的下降。在本试验中,棉籽浓缩蛋白全部替代饲料鱼粉(CPC组)亦对虹鳟幼鱼生长性能产生了明显的负面影响,导致其终终末体质量、WGR和SGR显著降低。已有研究显示,饲料中添加益生菌可改善肉食性鱼类的生长性能。如在饲料中同时添加枯草芽孢杆菌和地衣芽孢杆菌(Bacillus licheniformis)显著提高了虹鳟的终末体质量、WGR和SGR[15]。在基于豆粕的低鱼粉饲料(29.6%鱼粉)中添加枯草芽孢杆菌显著提高了虹鳟的WGR[13]。然而,也有一些研究结果表明饲料中添加益生菌对肉食性鱼类的生长没有明显的促进作用。Merrifield等[14]研究显示,在饲料中同时添加枯草芽孢杆菌和地衣芽孢杆菌对虹鳟的生长情况没有显著影响。本试验的研究结果也表明,在棉籽浓缩蛋白饲料中添加枯草芽孢杆菌对虹鳟幼鱼生长性能没有显著影响。不同研究结果的差异可能与饲料配方中植物蛋白质源的种类及添加比例、添加益生菌的种类和添加量以及试验鱼规格的不同有关。
Ji等[20]研究表明,在基于豆粕的饲料(42.8%鱼粉)中添加0.2% β-葡聚糖显著提高了虹鳟的WGR和SGR。另一项研究也表明,饲料中添加0.5% β-葡聚糖显著提高了虹鳟的WGR和SGR[21]。本试验的研究结果显示,在棉籽浓缩蛋白饲料中添加β-葡聚糖对虹鳟幼鱼生长性能没有明显的促进作用,这可能与本试验中棉籽浓缩蛋白替代饲料中鱼粉的比例过高有关。

3.2 棉籽浓缩蛋白饲料添加枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼血清生化指标的影响

血液是营养物质交换的主要场所,当机体受到外源因素影响时,血液指标也会发生相应改变,因而可以较好地指示机体产生的生理变化。血清ALT活性被认为是肝脏健康和新陈代谢的典型指标,当肝细胞受损后,ALT从细胞扩散进入血液,导致血清ALT活性升高[31]。Liu等[11]研究表明,高比例棉籽蛋白替代饲料鱼粉会导致虹鳟幼鱼血清ALT活性显著升高。本试验亦显示出相似的研究结果,即CPC组虹鳟幼鱼血清ALT活性显著高于CON组。但当在棉籽蛋白饲料中添加枯草芽孢杆菌和β-葡聚糖后,血清ALT活性显著下降,这表明枯草芽孢杆菌和β-葡聚糖具有保护虹鳟幼鱼肝脏健康的作用。相似的结果也在珍珠龙胆石斑鱼的研究中得到证明,即饲料(25%鱼粉和37%鱼粉)中添加枯草芽孢杆菌和β-葡聚糖均可显著降低其血清ALT活性[17,24]
LSZ是一种能够水解细菌中黏多糖的碱性酶,主要作用于革兰氏阳性菌,是机体吞噬细胞杀灭病原的物质基础[32]。Merrifield等[14]研究表明,在饲料中同时添加枯草芽孢杆菌和地衣芽孢杆菌显著提高了虹鳟血清LSZ活性。Newaj-Fyzul等[33]也证明了枯草芽孢杆菌可以提高虹鳟血清LSZ活性。这与本试验的结果类似,在棉籽蛋白饲料中添加枯草芽孢杆菌显著提高了虹鳟幼鱼血清LSZ活性。Khanjani等[21]研究表明,β-葡聚糖可以提高虹鳟血清LSZ活性。Ji等[20]研究表明,β-葡聚糖可以让感染杀鲑气单胞菌的虹鳟血清LSZ活性显著升高。本试验研究结果与上述结果类似,在棉籽浓缩蛋白饲料中添加枯草芽孢杆菌和β-葡聚糖均显著提高了虹鳟幼鱼血清LSZ活性,增强了无鱼粉饲料喂养虹鳟的免疫能力。

3.3 棉籽浓缩蛋白饲料添加枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道消化酶活性的影响

已有研究表明,植物蛋白质源饲料替代肉食性鱼类饲料中的鱼粉可导致其肠道消化酶活性降低。棉粕替代饲料中40%的鱼粉会致使花鲈(Lateolabrax japonicus)肠道淀粉酶和脂肪酶活性下降[34]。用发酵豆粕替代10%~40%的鱼粉喂养大口黑鲈[35],导致其肠道蛋白酶、脂肪酶和淀粉酶活性均呈现随替代比例升高而降低的趋势。本试验也呈现出相似的研究结果,棉籽浓缩蛋白完全替代饲料中鱼粉会导致虹鳟幼鱼肠道脂肪酶和α-淀粉酶活性显著降低。而枯草芽孢杆菌可以分泌多种胞外酶,包括淀粉酶、脂肪酶和蛋白酶,且在动物肠道酸性条件下具有很强的稳定性[36]。李军亮等[37]研究表明,在低鱼粉饲料中添加枯草芽孢杆菌对珍珠龙胆石斑鱼肠道淀粉酶和蛋白酶活性有促进作用。在本试验中,棉籽浓缩蛋白饲料添加枯草芽孢杆菌显著提高了虹鳟幼鱼肠道脂肪酶和α-淀粉酶活性。这与之前的研究结果类似,其原因可能是枯芽孢杆菌提供了外源性消化酶,从而促进了肠道对营养物质的吸收。王万良等[38]研究表明,在饲料中添加0.3% β-葡聚糖可以提高亚东鲑(Salmon trutta)幼鱼的肠道淀粉酶和脂肪酶活性。也有研究发现,在饲料中添加100 mg/kg的β-葡聚糖显著提高了珍珠龙胆石斑鱼肠道淀粉酶活性[24]。本试验中,棉籽浓缩蛋白饲料添加1.0% β-葡聚糖提高了虹鳟幼鱼肠道脂肪酶和淀粉酶活性,其原因可能与β-葡聚糖能够改善动物肠道菌群结构、促进营养物质代谢有关。

3.4 棉籽浓缩蛋白饲料添加枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肠道健康的影响

SOD、GSH-Px和CAT是鱼体主要的酶促抗氧化防御系统,SOD可以将超氧阴离子( O 2 -)转变为过氧化氢(H2O2),H2O2在GSH-Px的作用下进一步被催化分解,从而清除自由基;而MDA则可以作为间接反映机体氧化损伤程度的一个重要指标[23]。Li等[39]和He等[30]研究表明,高比例的棉籽蛋白替代饲料鱼粉会导致大口黑鲈肠道CAT和SOD活性显著降低,并提高肠道MDA含量。本试验中,CPC组虹鳟幼鱼肠道CAT活性显著低于CON组,且肠道MDA含量显著高于CON组,这与之前的研究结果类似。同时,棉籽浓缩蛋白饲料添加枯草芽孢杆菌提高了虹鳟幼鱼肠道CAT活性和T-AOC,降低了肠道MDA含量,且Ⅱ组肠道CAT、SOD和GSH-Px活性相比于Ⅰ组和Ⅲ组更高,说明枯草芽孢杆菌随饲料进入鱼体后可能通过自身分泌抗氧化酶或者作为激活剂促进机体抗氧化酶分泌,从而有效清除自由基,阻止脂质过氧化[40]。Park等[13]研究表明,饲料中添加枯草芽孢杆菌可以提高虹鳟肠道SOD活性。Taherpour等[41]研究也表明,枯草芽孢杆菌可以提高虹鳟肝脏CAT和SOD活性。张冬梅等[16]研究表明,1.0%枯草芽孢杆菌组大口黑鲈肠道总超氧化物歧化酶(T-SOD)、CAT和GSH-Px活性显著高于对照组和0.5%枯草芽孢杆菌组,肠道MDA含量显著低于对照组。
研究表明,肉食性鱼类饲料中添加β-葡聚糖对肠道抗氧化能力具有提升作用。例如,β-葡聚糖显著提高了感染杀鲑气单胞菌虹鳟的血清T-AOC和GSH-Px活性,并降低了血清MDA含量[42-43]。Ji等[20]研究也表明,虹鳟感染杀鲑气单胞菌后,β-葡聚糖组血清T-SOD和CAT活性更高。Tkachenko等[44]研究表明,β-葡聚糖可以提高虹鳟肝脏CAT和GSH-Px活性。本试验结果与之前研究结果类似,棉籽浓缩蛋白饲料添加β-葡聚糖提高了虹鳟肠道T-AOC以及SOD和CAT活性,且添加1.0% β-葡聚糖相比于添加0.1% β-葡聚糖效果更好;同时,棉籽浓缩蛋白饲料添加1.0% β-葡聚糖也显著降低了血清MDA含量。研究结果表明,β-葡聚糖可以在虹鳟无鱼粉饲料中发挥积极作用,催化肠道组织的 O 2 -生成H2O2以清除自由基,降低机体氧化损伤。
细胞因子在脊椎动物免疫系统的调节中发挥着重要作用,已被用作评估肠道健康的标志物[45]。已有研究表明,棉籽蛋白高比例替代饲料鱼粉会导致虹鳟、大口黑鲈等肉食性鱼类肠道促炎因子(IL-1βIL-8、TNF-α)表达量的显著升高[11,30,39]。本试验中,棉籽浓缩蛋白完全替代饲料中的鱼粉也显著上调了虹鳟幼鱼肠道促炎因子(IL-1βIL-8、TNF-α)mRNA相对表达量。研究表明,饲料中添加枯草芽孢杆菌可以调控肉食性鱼类肠道炎性因子基因表达。例如,Panigrahi等[46]报道,饲料中加入枯草芽孢杆菌显著提高了虹鳟肾脏中TGF-β mRNA相对表达量。研究还表明,枯草芽孢杆菌显著降低大口黑鲈幼鱼肠道促炎因子IL-1β、白细胞介素-15(IL-15)、TNF-αIL-8的mRNA相对表达量,并显著提高了抗炎因子IL-10和TGF-β1的mRNA相对表达量[16]。本研究也得到了相似的结果,在棉籽浓缩蛋白饲料中添加枯草芽孢杆菌可以显著降低虹鳟幼鱼肠道促炎因子(IL-1βIL-8、TNF-α)mRNA相对表达量,并显著提高抗炎因子TGF-βIL-10 mRNA相对表达量,且Ⅱ组效果更好。
现有研究显示,饲料中添加β-葡聚糖可以调控虹鳟肠道炎性因子基因表达,改善肠道健康状况[47-48]。本试验的研究结果也表明,棉籽蛋白饲料添加β-葡聚糖可以下调促炎因子基因表达。此外,棉籽浓缩蛋白饲料添加枯草芽孢杆菌和1.0% β-葡聚糖均可以显著提高虹鳟幼鱼肠道C3和C4 mRNA相对表达量。C3和C4作为补体系统的成员,在机体防御过程中可通过免疫复合物、调理吞噬细胞等机制对病原微生物进行清除,以及活化炎性细胞对靶细胞的杀伤作用[49-50],并可以调控炎性因子的表达[18,51-52]
紧密连接蛋白是一种屏障蛋白,在鱼类肠道屏障中发挥着重要作用,可防止细菌、脂多糖和其他潜在有害物质进入血液[53]。紧密连接蛋白连接在相邻的上皮细胞之间形成了由跨膜蛋白如封闭蛋白(claudin)和闭合蛋白(occludin)和胞质蛋白如ZO-1所维持的复杂蛋白质结构[54]。CLD1与肠上皮细胞通透性密切相关,其表达的变化直接反映肠道黏膜机械屏障的变化[55]。在氧化应激和还原条件下,OCLN被确定为最敏感的紧密连接蛋白和潜在的紧密连接调节蛋白[56],OCLN的降低会导致肠道黏膜屏障受损,影响其免疫功能[57]。ZO-1的主要功能是连接紧密连接蛋白与细胞骨架,从而形成稳定的紧密连接复合体[58]。有研究表明,棉籽蛋白替代鱼粉时,会显著降低大口黑鲈肠道CLD1、OCLNZO-1 mRNA相对表达量[30]。这与本试验的研究结果相似,CPC组虹鳟幼鱼肠道CLD1、OCLNTRICZO-1 mRNA相对表达量显著低于CON组,说明高比例的棉籽浓缩蛋白替代饲料鱼粉对肠道紧密连接蛋白的功能造成损伤。本试验中,与CPC组相比,Ⅱ组和Ⅴ组虹鳟幼鱼肠道OCLNZO-1的mRNA相对表达量均显著提高。同时,肠道组织学的结果显示,棉籽蛋白饲料添加枯草芽孢杆菌可以提高虹鳟幼鱼肠道绒毛高度和肌层厚度。以上的研究结果也证实了枯草芽孢杆菌和β-葡聚糖对于高棉籽浓缩蛋白饲料饲喂引起的虹鳟肠道损伤具有明显地缓解作用。

3.5 棉籽浓缩蛋白饲料添加枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼肝脏和脾脏抗病力的影响

杀鲑气单胞菌为革兰氏阴性短杆菌,属于气胞菌科、气胞菌属,有鞭毛,无运动能力[59]。该菌具有广泛的地理分布,且具有较强的致病性,对很多国家的养殖鱼类造成了严重的冲击,尤其是经济价值较高的鲑科鱼类[60]。已有研究表明,枯草芽孢杆菌可以通过增强细胞免疫和体液免疫来增强鱼类的抗病性[61]。例如,枯草芽孢杆菌可以增强虹鳟对杀鲑气单胞菌的抵抗力,包括刺激免疫参数,特别是通过提升血清LSZ和抗氧化酶活性来提高虹鳟感染杀鲑气单胞菌后的存活率[13,33],这与本试验的结果类似。另有研究结果显示,β-葡聚糖可以显著提升虹鳟抗杀鲑气单胞菌的能力,通过调节杀鲑气单胞菌感染期间的生物化学过程、细胞因子、免疫因素以及激活Toll样受体(TLR)和细胞外信号调节激酶(ERK)信号通路,有效降低累积死亡率[20,43,62]。本试验的研究结果表明,棉籽浓缩蛋白饲料添加枯草芽孢杆菌和β-葡聚糖均可显著降低虹鳟肝脏和脾脏组织的鲑气单胞菌数量,提升虹鳟抗杀鲑气单胞菌的能力,说明枯草芽孢杆菌和β-葡聚糖可以显著改善因高比例棉籽浓缩蛋白添加导致的虹鳟抗病力下降的问题。

4 结论

棉籽浓缩蛋白饲料添加枯草芽孢杆菌和β-葡聚糖对虹鳟幼鱼生长性能没有明显的促进作用,但显著改善了部分血清生化指标,提升了肠道健康水平以及抗杀鲑气单胞菌的能力,且以喷涂方式添加1×10⁸ CFU/g枯草芽孢杆菌和添加1.0% β-葡聚糖对虹鳟幼鱼的效果较佳。
[1]
Food and Agriculture Organization of the United Nations. The state of world fisheries and aquaculture 2022[M]. Rome:FAO, 2022.

[2]
冷向军. 低鱼粉水产饲料的研究与应用[J]. 饲料工业, 2020, 41(22):1-8.

LENG X J. The research and application of low fish meal diets in aquaculture[J]. Feed Industry, 2020, 41(22):1-8. (in Chinese)

[3]
陆阳, 杨雨虹, 王裕玉, 等. 不同比例膨化豆粕替代鱼粉对虹鳟生长、体成分及血液学指标的影响[J]. 动物营养学报, 2010, 22(1):221-227.

LU Y, YANG Y H, WANG Y Y, et al. Effects of different replacement ratio of fish meal by extruded soybean meal on growth,body composition and hematology indices of rainbow trout (Oncorhynchus mykiss)[J]. Chinese Journal of Animal Nutrition, 2010, 22(1):221-227. (in Chinese)

[4]
胡俊茹, 蓝青, 张春燕, 等. 发酵豆粕替代鱼粉对大口黑鲈生长、生化指标及肠道健康的影响[J]. 饲料工业, 2023, 44(2):66-76.

HU J R, LAN Q, ZHANG C Y, et al. Effects of fish meal replacement with fermented soybean meal on growth, serum biochemical indices and intestinal health of largemouth bass (Micropterus salmoides)[J]. Feed Industry, 2023, 44(2):66-76. (in Chinese)

[5]
薛敏. 棉籽浓缩蛋白加工工艺及其在水产饲料中营养价值[J]. 饲料工业, 2021, 42(12):1-5.

XUE M. Processing of cottonseed protein concentrated and its nutrient values in aquatic feed[J]. Feed Industry, 2021, 42(12):1-5. (in Chinese)

[6]
XU X, YANG H, ZHANG C, et al. Effects of replacing fishmeal with cottonseed protein concentrate on growth performance,flesh quality and gossypol deposition of largemouth bass (Micropterus salmoides)[J]. Aquaculture, 2022,548:737551.

[7]
XIE X, WANG J, GUAN Y, et al. Cottonseed protein concentrate as fishmeal alternative for largemouth bass (Micropterus salmoides) supplemented a yeast-based paraprobiotic:effects on growth performance,gut health and microbiome[J]. Aquaculture, 2022,551:737898.

[8]
赵小龙, 刘大川. 棉籽蛋白资源开发研究进展[J]. 中国油脂, 2014, 39(1):23-26.

ZHAO X L, LIU D C. Progress on cottonseed protein resource[J]. China Oils and Fats, 2014, 39(1):23-26. (in Chinese)

[9]
ZHAO W, LIU Z L, NIU J. Growth performance,intestinal histomorphology,body composition,hematological and antioxidant parameters of Oncorhynchus mykiss were not detrimentally affected by replacement of fish meal with concentrated dephenolization cottonseed protein[J]. Aquaculture Reports, 2021,19:100557.

[10]
LUO L, XUE M, WU X, et al. Partial or total replacement of fishmeal by solvent-extracted cottonseed meal in diets for juvenile rainbow trout (Oncorhynchus mykiss)[J]. Aquaculture Nutrition, 2006, 12(6):418-424.

[11]
LIU Y, MA S W, LV W H, et al. Effects of replacing fishmeal with cottonseed protein concentrate on growth performance,blood metabolites,and the intestinal health of juvenile rainbow trout (Oncorhynchus mykiss)[J]. Frontiers in Immunology, 2022,13:1079677.

[12]
苏艳莉, 孙盛明, 朱健, 等. 枯草芽孢杆菌在水产养殖中的研究进展[J]. 中国渔业质量与标准, 2016, 6(6):32-39.

SU Y L, SUN S M, ZHU J, et al. Advances of Bacillus subtilis application in aquaculture[J]. China Fishery Quality and Standards, 2016, 6(6):32-39. (in Chinese)

[13]
PARK Y, LEE S, HONG J, et al. Use of probiotics to enhance growth,stimulate immunity and confer disease resistance to Aeromonas salmonicida in rainbow trout (Oncorhynchus mykiss)[J]. Aquaculture Research, 2017, 48(6):2672-2682.

[14]
MERRIFIELD D L, DIMITROGLOU A, BRADLEY G, et al. Probiotic applications for rainbow trout (Oncorhynchus mykiss Walbaum) Ⅰ.Effects on growth performance,feed utilization,intestinal microbiota and related health criteria[J]. Aquaculture Nutrition, 2010, 16(5):504-510.

[15]
NARAGHI M, SHAMSAIE MEHRGAN M, MANOUCHEHRI H. Dietary incorporation of Bacillus subtilis and Bacillus licheniformis mixture (DiPro Aqua) ameliorates growth performance,immune response,and intestinal morphology in rainbow trout[J]. North American Journal of Aquaculture, 2022,84:116-125.

[16]
张冬梅, 颜浩骁, 罗茂林, 等. 饲料中添加枯草芽孢杆菌对大口黑鲈幼鱼生长、肠道组织结构、抗氧化能力、免疫能力和肠炎的影响[J]. 动物营养学报, 2022, 34(1):575-588.

DOI

ZHANG D M, YAN H X, LUO M L, et al. Effects of dietary Bacillus subtilis on growth,intestinal tissue structure,antioxidant capacity,immunity and enteritis of juvenile largemouth bass (Micropterus salmoides)[J]. Chinese Journal of Animal Nutrition, 2022, 34(1):575-588. (in Chinese)

[17]
王成强, 李宝山, 王际英, 等. 饲料中添加枯草芽孢杆菌和酵母培养物对珍珠龙胆石斑鱼幼鱼生长、血清生化指标及抗氧化能力的影响[J]. 渔业科学进展, 2019, 40(4):47-56.

WANG C Q, LI B S, WANG J Y, et al. Effects of dietary Bacillus subtilis and yeast culture on growth,serum biochemical indices and antioxidant capacity of juvenile hybrid grouper (Epinephelus fuscoguttatus♀×E. lanceolatus♂)[J]. Progress in Fishery Sciences, 2019, 40(4):47-56. (in Chinese)

[18]
曹俊明, 赵红霞, 黄燕华, 等. β-葡聚糖及其在水生动物中的应用研究[J]. 饲料工业, 2013(18):1-6.

CAO J M, ZHAO H X, HUANG Y H, et al. β-glucan and its application in aquatic animals[J]. Feed Industry, 2013(18):1-6. (in Chinese)

[19]
王银东, 何吉祥. β-葡聚糖的来源、特性及在水产动物中的应用[J]. 长江大学学报(自科版), 2014, 11(4):30-34,38.

WANG Y D, HE J X. Sources,properties and application of β-glucan in aquatic animals[J]. Journal of Yangtze University (Natural Science Edition), 2014, 11(4):30-34,38. (in Chinese)

[20]
JI L Q, SUN G X, LI J, et al. Effect of dietary β-glucan on growth,survival and regulation of immune processes in rainbow trout (Oncorhynchus mykiss) infected by Aeromonas salmonicida[J]. Fish & Shellfish Immunology, 2017,64:56-67.

[21]
KHANJANI M H, GHAEDI G, SHARIFINIA M. Effects of diets containing β-glucan on survival,growth performance,haematological,immunity and biochemical parameters of rainbow trout (Oncorhynchus mykiss) fingerlings[J]. Aquaculture Research, 2022, 53(5):1842-1850.

[22]
SEALEY W M, BARROWS F T, HANG A, et al. Evaluation of the ability of barley genotypes containing different amounts of β-glucan to alter growth and disease resistance of rainbow trout Oncorhynchus mykiss[J]. Animal Feed Science and Technology, 2007, 141(1/2):115-128.

[23]
胡俊茹, 朱喜锋, 李国立, 等. β-葡聚糖对大口黑鲈生长、体组成和抗氧化能力的影响[J]. 淡水渔业, 2023, 53(2):43-49.

HU J R, ZHU X F, LI G L, et al. Effects of dietary β-glucan on growth,body composition and antioxidant capacity of largemouth bass (Micropterus salmoides)[J]. Freshwater Fisheries, 2023, 53(2):43-49. (in Chinese)

[24]
陈俭, 代冰涛, 王红明, 等. 饲料中添加β-葡聚糖对珍珠龙胆石斑鱼生长性能、免疫指标、转录组及肠道菌群的影响[J]. 南方农业学报, 2022, 53(5):1434-1447.

CHEN J, DAI B T, WANG H M, et al. Effects of adding β-glucan to feed on the growth performance,immune indexes,transcriptome and intestinal flora of Epinephelus fuscoguttatus♀×Epinephelus lanceolatus♂[J]. Journal of Southern Agriculture, 2022, 53(5):1434-1447. (in Chinese)

[25]
JOBLING M. National Research Council (NRC):nutrient requirements of fish and shrimp[J]. Aquaculture International, 2012,20:601-602.

[26]
樊丹, 邓福容, 李绍戊, 等. 一株虹鳟源枯草芽孢杆菌的分离鉴定及生物学特性研究[J]. 中国海洋大学学报(自然科学版), 2022, 52(2):41-49.

FAN D, DENG F R, LI S W, et al. Isolation,identification and biological characterization of a Bacillus subtilis strain from rainbow trout (Oncorhynchus mykiss)[J]. Periodical of Ocean University of China (Natural Science Edition), 2022, 52(2):41-49. (in Chinese)

[27]
HUYBEN D, VIDAKOVIC A, SUNDH H, et al. Haematological and intestinal health parameters of rainbow trout are influenced by dietary live yeast and increased water temperature[J]. Fish & Shellfish Immunology, 2019,89:525-536.

[28]
LIVAK K J, SCHMITTGEN T D. Analysis of relative gene expression data using real-time quantitative PCR and the 2-ΔΔCt method[J]. Methods, 2001, 25(4):402-408.

[29]
申建飞, 陈铭灿, 刘泓宇, 等. 浓缩棉籽蛋白替代鱼粉对卵形鲳鲹幼鱼生长性能、血清生化指标、肝脏抗氧化指标及胃肠道蛋白酶活性的影响[J]. 动物营养学报, 2019, 31(2):746-756.

SHEN J F, CHEN M C, LIU H Y, et al. Effects of fish meal replacement by concentrated cottonseed protein on growth performance,serum biochemical indices,liver antioxidant indices and gastrointestinal tract protease activities of juvenile Trachinotus ovatus[J]. Chinese Journal of Animal Nutrition, 2019, 31(2):746-756. (in Chinese)

[30]
HE G, ZHANG T, ZHOU X, et al. Effects of cottonseed protein concentrate on growth performance,hepatic function and intestinal health in juvenile largemouth bass,Micropterus salmoides[J]. Aquaculture Reports, 2022,23:101052.

[31]
KIM W R, FLAMM S L, DI BISCEGLIE A M, et al. Serum activity of alanine aminotransferase (ALT) as an indicator of health and disease[J]. Hepatology (Baltimore,Md.), 2008, 47(4):1363-1370.

[32]
RAGLAND S A, CRISS A K. From bacterial killing to immune modulation:recent insights into the functions of lysozyme[J]. PLoS Pathogens, 2017, 13(9):e1006512.

[33]
NEWAJ-FYZUL A, ADESIYUN A A, MUTANI A, et al. Bacillus subtilis AB1 controls Aeromonas infection in rainbow trout (Oncorhynchus mykiss,Walbaum)[J]. Journal of Applied Microbiology, 2007, 103(5):1699-1706.

[34]
王国霞, 付晶晶, 黄燕华, 等. 5种植物蛋白源替代鱼粉对花鲈生长性能和消化酶活性的影响[J]. 湖北农业科学, 2014, 53(4):866-870.

WANG G X, FU J J, HUANG Y H, et al. Effects of partial replacement of fish meal by five plant proteins on growth performance and digestive enzymes activities of Lateolabrax japonicus[J]. Hubei Agricultural Sciences, 2014, 53(4):866-870. (in Chinese)

[35]
田鑫鑫, 黄卫, 谢春元, 等. 发酵豆粕替代鱼粉对大口黑鲈幼鱼生长、饲料利用和消化酶活力的影响[J]. 上海海洋大学学报, 2022, 31(2):355-364.

TIAN X X, HUANG W, XIE C Y, et al. Effects of fermented soybean meal replacing of fish meal on the growth,feed utilization and digestive enzyme activity of juvenile largemouth bass (Micropterus salmoides)[J]. Journal of Shanghai Ocean University, 2022, 31(2):355-364. (in Chinese)

[36]
KUEBUTORNYE F K A, ABARIKE E D, LU Y. A review on the application of Bacillus as probiotics in aquaculture[J]. Fish & Shellfish Immunology, 2019,87:820-828.

[37]
李军亮, 杨奇慧, 谭北平, 等. 低鱼粉饲料添加枯草芽孢杆菌对珍珠龙胆石斑鱼幼鱼生长、消化酶活性、抗氧化酶活性及其mRNA表达的影响[J]. 水产学报, 2019, 43(4):1126-1137.

LI J L, YANG Q H, TAN B P, et al. Effect of low-fishmeal diet with Bacillus subtilis on growth performance,digestive enzyme activity,antioxidant enzyme activity and its mRNA expression of juveniles Epinephelus lanceolatu♂×Epinephelus fuscoguttatus♀[J]. Journal of Fisheries of China, 2019, 43(4):1126-1137. (in Chinese)

[38]
王万良, 周建设, 陈美群, 等. β-葡聚糖对亚东鲑幼鱼生长、肠道消化酶活性及肝脏抗氧化能力的影响[J]. 西南农业学报, 2021, 34(3):673-678.

WANG W L, ZHOU J S, CHEN M Q, et al. Effects of β-glucan on growth,intestinal digestive enzyme activity and liver antioxidant capacity of juvenile salmon trutta[J]. Southwest China Journal of Agricultural Sciences, 2021, 34(3):673-678. (in Chinese)

[39]
LI L, LIU X, WANG Y, et al. Effects of alternate feeding between fish meal and novel protein diets on the intestinal health of juvenile largemouth bass (Micropterus salmoides)[J]. Aquaculture Reports, 2022,23:101023.

[40]
沈文英, 李卫芬, 梁权, 等. 饲料中添加枯草芽孢杆菌对草鱼生长性能、免疫和抗氧化功能的影响[J]. 动物营养学报, 2011, 23(5):881-886.

SHEN W Y, LI W F, LIANG Q, et al. Effects of dietary Bacillus subtilis on growth performance,immunity and antioxidant function of grass carp (Ctenopharyngodon idellus)[J]. Chinese Journal of Animal Nutrition, 2011, 23(5):881-886. (in Chinese)

[41]
TAHERPOUR M, ROOMIANI L, ISLAMI H R, et al. Effect of dietary butyric acid,Bacillus licheniformis (probiotic),and their combination on hemato-biochemical indices,antioxidant enzymes,immunological parameters,and growth performance of Rainbow trout(Oncorhynchus mykiss)[J]. Aquaculture Reports, 2023,30:101534.

[42]
纪利芹, 孙国祥, 王艺, 等. β-葡聚糖对杀鲑气单胞菌感染后虹鳟应激过程的调节作用[J]. 中国水产科学, 2018, 25(1):178-188.

JI L Q, SUN G X, WANG Y, et al. Effect of different dietary β-glucan dosages on regulation of stress re-sponse in rainbow trout infected by Aeromonas salmonicida[J]. Journal of Fishery Sciences of China, 2018, 25(1):178-188. (in Chinese)

[43]
JI L Q, FU S Z, SUN G X, et al. Dietary β-glucan modulate haematological parameters,cytokines and gene expression in TLR and ERK pathways of rainbow trout (Oncorhynchus mykiss) during infection by Aeromonas salmonicida[J]. Aquaculture Research, 2020, 51(3):906-917.

[44]
TKACHENKO H, GRUDNIEWSKA J, KURHALUK N. Effects of dietary yeast β-1.3/1.6-glucans on oxidative stress biomarkers in hearts and livers of rainbow trout (Oncorhynchus mykiss Walbaum),European whitefish (Coregonus lavaretus L.),and grayling (Thymallus thymallus L.)[J]. Fisheries & Aquatic Life, 2022, 30(3):149-168.

[45]
SAKAI M, HIKIMA J I, KONO T. Fish cytokines:current research and applications[J]. Fisheries Science, 2021, 87(1):1-9.

[46]
PANIGRAHI A, KIRON V, SATOH S, et al. Immune modulation and expression of cytokine genes in rainbow trout Oncorhynchus mykiss upon probiotic feeding[J]. Developmental & Comparative Immunology, 2007, 31(4):372-382.

[47]
JI L, FU S, JI R, et al. β-glucan mitigated trinitrobenzene sulfonic acid-induced enteritis in the rainbow trout (Oncorhynchus mykiss)[J]. Aquaculture, 2019,513:734393.

[48]
LIU Y, CHANG H, HAN D, et al. Effects of dietary chrysophyte (Poterioochromonas malhamensis) rich in beta-glucan on the growth performance,intestinal health,lipid metabolism,immune gene expression,and disease resistance against Aeromonas salmonicida in juvenile rainbow trout (Oncorhynchus mykiss)[J]. Aquaculture, 2022,561:738589.

[49]
崔保安, 杨明凡, 张素梅, 等. 有机硒和某些中草药对鸡免疫功能的影响[J]. 畜牧与兽医, 2003, 35(10):37-38.

CUI B A, YANG M F, ZHANG S M, et al. Effect of organic Se and several Chinese herbal medicines on chicken immunity[J]. Animal Husbandry & Veterinary Medicine, 2003, 35(10):37-38. (in Chinese)

[50]
王超英, 柳纪省, 白银梅, 等. 鸡用天然缓释免疫增强剂的研究——天然免疫增效药物的筛选[J]. 中国兽医科技, 1998(7):13-15.

WANG C Y, LIU J S, BAI Y M, et al. Study of natural slow-release immune enhancers for chickens:screening of natural immune-enhancing drugs[J]. Chinese Journal of Veterinary Science and Technology, 1998(7):13-15. (in Chinese)

[51]
TAKABAYASHI T, VANNIER E, CLARK B D, et al. A new biologic role for C3a and C3a desArg:regulation of TNF-alpha and IL-1 beta synthesis[J]. Journal of Immunology, 1996, 156(9):3455-3460.

[52]
HAEFFNER-CAVAILLON N, CAVAILLON J M, LAUDE M, et al. C3a (C3adesArg) induces production and release of interleukin 1 by cultured human monocytes[J]. Journal of Immunology (Baltimore,Md.: 1950),1987, 139(3):794-799.

[53]
LIU Z T, QUE S P, XU J, et al. Alanine aminotransferase-old biomarker and new concept:a review[J]. International Journal of Medical Sciences, 2014, 11(9):925-935.

[54]
孔瑶瑶, 马秀华, 麦康森, 等. 饲料营养素对鱼类肠道紧密连接蛋白闭锁小带蛋白-1影响的研究进展[J]. 动物营养学报, 2020, 32(11):5081-5088.

DOI

KONG Y Y, MA X H, MAI K S, et al. Research progress of effects of diet nutrients on intestinal tight junction protein zonula occludens-1 of fish[J]. Chinese Journal of Animal Nutrition, 2020, 32(11):5081-5088. (in Chinese)

[55]
吴雪芹, 陈秀梅, 王桂芹, 等. 紧密连接蛋白在鱼类肠道屏障损伤中的研究进展[J]. 饲料工业, 2023, 44(6):56-62.

WU X Q, CHEN X M, WANG G Q, et al. A review on tight junction protein in fish intestinal barrier injury[J]. Feed Industry, 2023, 44(6):56-62. (in Chinese)

[56]
BLASIG I E, BELLMANN C, CORDING J, et al. Occludin protein family:oxidative stress and reducing conditions[J]. Antioxidants & Redox Signaling, 2011, 15(5):1195-1219.

[57]
AL-SADI R, KHATIB K, GUO S H, et al. Occludin regulates macromolecule flux across the intestinal epithelial tight junction barrier[J]. American Journal of Physiology:Gastrointestinal and Liver Physiology, 2011, 300(6):G1054-G1064.

[58]
SUZUKI T. Regulation of intestinal epithelial permeability by tight junctions[J]. Cellular and Molecular Life Sciences:CMLS, 2013, 70(4):631-659.

[59]
李联泰, 卫明亮, 刘煜恒, 等. 杀鲑气单胞菌疫苗的研制[J]. 江苏海洋大学学报(自然科学版), 2020, 29(2):1-5.

LI L T, WEI M L, LIU Y H, et al. Development of Aeromonas salmonucuda vaccine[J]. Journal of Jiangsu Ocean University (Natural Sciences Edition), 2020, 29(2):1-5. (in Chinese)

[60]
张晓君. 三种海水养殖鱼类的主要细菌性疾病研究[D]. 博士学位论文. 青岛: 中国海洋大学, 2006.

ZHANG X J. Studies on the main bacterial diseases in 3 marine fish[D]. Ph.D. Thesis. Qingdao: Ocean University of China, 2006. (in Chinese)

[61]
NAYAK S K. Probiotics and immunity:a fish perspective[J]. Fish & Shellfish Immunology, 2010, 29(1):2-14.

[62]
JI L Q, SUN G X, LI X, et al. Comparative transcriptome analysis reveals the mechanism of β-glucan in protecting rainbow trout (Oncorhynchus mykiss) from Aeromonas salmonicida infection[J]. Fish & Shellfish Immunology, 2020,98:87-99.

Outlines

/