RESEARCH PAPER

Effects of Piper sarmentosum Roxb. Extract on Testicular Growth and Development, Antioxidant Capacity and Immune Level of Hainan Black Goats under Summer

  • CHEN Yixin , 1, 2 ,
  • YANG Tingshuo 1, 2, * ,
  • REN Guodong 1, 2 ,
  • SHENG Ziyang 1, 2 ,
  • ZHANG Nan 1, 2 ,
  • ZHOU Hanlin 3, 4 ,
  • WANG Dingfa 4 ,
  • LYU Renlong 4 ,
  • LUO Hailing , 1, 2, **
Expand
  • 1 Sanya Institute of China Agricultural University, Sanya 572025, China
  • 2 State Key Laboratory of Animal Nutrition and Feeding, College of Animal Science and Technology, China Agricultural University, Beijing 100193, China
  • 3 Zhanjiang Experimental Station, Chinese Academy of Tropical Agricultural Sciences, Zhanjiang 524019, China
  • 4 Tropical Crops Genetic Resources Institute, Chinese Academy of Tropical Agricultural Sciences, Haikou 571101, China
**professor, E-mail:

*Contributed equally

Received date: 2024-03-02

  Online published: 2024-10-14

Abstract

The aim of this study was to investigate the effects of Piper sarmentosum Roxb. extract (PSE) on the testicular growth and development, hormone level, antioxidant capacity and immune level of Hainan black goats in summer. Thirty-six 3-month-old healthy Hainan black goat male lambs with similar body weight were selected for the experiment and randomly divided into four groups of nine lambs each using a one-way completely randomized experimental design, and each lamb was raised in a single pen. Lambs were fed basal diets supplemented with 0 (CON group), 200 (200PSE group), 400 (400PSE group) and 600 mg/kg PSE (600PSE group), respectively. The pre-trial period lasted for 15 days and the experimental period lasted for 90 days. The results showed that the diets supplemented with different levels of PSE did not significantly affect the growth and development of scrotum, testis and epididymis of Hainan black goats in summer (P>0.05). Compared with the CON group, when diets supplemented with 200, 400 and 600 mg/kg PSE, the testis weight was increased by 10.73%, 4.26% and 8.58%, and the epididymis weight was increased by 24.82%, 36.04% and 32.46%, respectively. The seminiferous tubule diameter of the 400PSE group and 600PSE group was significantly increased compared with the CON group and 200PSE group (P<0.05); except interstitial cells, the densities of other spermatogenic cells (Sertoli cells, spermatogonia, spermatocyte, sperm cells, and sperm) in the seminiferous tubule of 400PSE group had the highest values, and were significantly higher than those of CON group (P<0.05). The levels of testosterone (T) and luteinizing hormone (LH) in testicular tissue had the highest values in the 600PSE group, and had the lowest values in the 400PSE group, there were significant differences between 600PSE group and 400PSE group (P<0.05); compared with the CON group, the succinate dehydrogenase (SDH) activity in testicular tissue of 400PSE group was significantly increased (P<0.05). The total antioxidant capacity (T-AOC) in testicular tissue of 400PSE group and 600PSE group was significantly increased compared with the CON group (P<0.05); the superoxide dismutase (SOD) activity in testicular tissue of 200PSE group, 400PSE group and 600PSE group was significantly increased compared with the CON group (P<0.05), and they were increased by 14.11%, 23.45% and 17.20%, respectively; compared with the CON group, the content of immunoglobulin G (IgG) in testicular tissue of 200PSE group, 400PSE group and 600PSE group was increased by 9.73% (P<0.05), 4.18% (P>0.05) and 10.83% (P<0.05), and the content of interleukin-4 (IL-4) was increased by 7.56% (P>0.05), 2.66% (P>0.05) and 15.46% (P<0.05), respectively; the content of heat shock protein 27 (HSP27) in testicular tissue was significantly increased when the supplemental level of PES was 600 mg/kg (P<0.05). In conclusion, diet supplemented with PSE can increase the antioxidant capacity and immune level of testicular tissue, alleviate the potential oxidative damage of testis induced by heat stress, and then promote the testicular growth and development of Hainan black goats under summer.

Cite this article

CHEN Yixin , YANG Tingshuo , REN Guodong , SHENG Ziyang , ZHANG Nan , ZHOU Hanlin , WANG Dingfa , LYU Renlong , LUO Hailing . Effects of Piper sarmentosum Roxb. Extract on Testicular Growth and Development, Antioxidant Capacity and Immune Level of Hainan Black Goats under Summer[J]. Chinese Journal of Animal Nutrition, 2024 , 36(10) : 6494 -6510 . DOI: 10.12418/CJAN2024.552

随着全球气候变化加剧,世界各地区面临着日益频繁和严重的干旱问题,这对全球畜禽生产构成严重威胁,环境问题俨然已迅速成为畜牧生产从业者又一大关注热点[1]。环境应激源,如热应激,对畜牧业尤其有害[2]。热应激是指从动物体内流向周围环境的能量少于动物产生的能量,这是环境因素(如阳光、热辐射、空气温度和相对湿度)变化和动物自身特性(如物种、新陈代谢率和体温调节机制)造成的,进而对动物机体所产生的一系列损伤的应激过程[3]。当前,各种温度评估指数,如温湿度指数(temperature humidity index,THI)、热负荷指数、等效温度指数、呼吸频率和环境压力指数等,被用于评估动物热应激状态[4],其中THI是被广泛用作评估畜禽生产中热应激的重要环境评估指标[5]。研究证明,热应激会对动物生长[6]、产奶量[7]、产肉量[8]等生产性能产生不利影响。此外,下丘脑-垂体-肾上腺轴也可响应热应激而被激活,进而影响生长激素的释放,对生长产生负面影响[9]。即便对于具有热适应性的动物而言,在热应激影响下生长速度、产奶量和产肉量也有不同程度降低[10-12]。热应激不仅损害畜禽生产,还会对雄性动物生殖器官及功能造成影响。睾丸作为雄性动物的生殖器官,主要作用是分泌雄性激素睾酮并生成精子,其受到睾丸体细胞(支持细胞和间质细胞)和生殖细胞的正常发育来调控[13]。睾丸温度比机体核心体温低2~7 ℃,并且通过特殊的热交换机制保持较低的温度,这样可以确保正常精子的产生[14-15]。热应激对雄性动物生殖器官及功能的影响包括精子数量和质量下降、激素水平改变、睾丸损伤和炎症反应,这可能导致生殖能力下降和生殖功能障碍。研究表明,热应激诱导的氧化应激会导致豚鼠[16]、猪[17]、山羊[18]和奶牛[19]雄性腔体的生殖器官重量降低,影响血清生化指标,并引起睾丸结构和功能受损。
假蒟(Piper sarmentosum Roxb.)是一种多年生草本植物,属于胡椒属,广泛分布于东南亚国家和我国东南沿海地区,包括广东省、福建省和海南省等[20-22]。几个世纪以来,假蒟被当作“药食同源”类植物。假蒟整株,包括叶片和根部,既是一种可食用的蔬菜,也是一种传统的药用草药,用途广泛,可治疗如感冒、发烧、牙痛甚至抑郁等各种疾病[23-25]。在对假蒟药理作用的进一步探究中发现,假蒟具有抗过敏、抗炎和抗动脉粥样硬化的潜力[26-28]。假蒟及其提取物含有丰富的挥发油、生物碱和黄酮类等活性物质[29]。陈川威等[30]采用石油醚、乙酸乙酯和正丁醇3种不同介质分别对假蒟进行提取,发现得到的3种提取物都有较强的抗氧化能力。在饲粮中添加50 mg/kg假蒟提取物(Piper sarmentosum Roxb. extract,PSE)能提高断奶仔猪的日采食量和免疫力,促进蛋白质的合成与代谢[31];此外,有研究发现,在基础饲粮中添加50或200 mg/kg的PSE,能够提高68周海南文昌鸡的日增重和日采食量,并改善胸肌肉品质[32]
由于海南岛特殊的热带地理环境,海南黑山羊在夏季有面临高热应激的风险,这容易导致海南黑山羊产生应激而影响生殖性能,大大增加了海南黑山羊的生产繁殖周期。如何有效改善其生产性能、缩短生产周期和缓解环境带来的应激成为海南养羊业广泛关注的问题。本团队前期研究证明PSE可以显著提高海南黑山羊体外瘤胃发酵的产气量、pH与体外干物质消化率,并使发酵模式由乙酸发酵转向丙酸发酵,因而提高能量利用效率[33];在海南炎热夏季,饲粮中添加不同水平PSE显著降低了海南黑山羊的料重比,提高其对饲粮中干物质、中性洗涤纤维和酸性洗涤纤维的表观消化率,提高了饲料利用效率,并显著提高了抗氧化能力[34]。因此,本试验旨在探究PSE对夏季海南黑山羊公羔生殖器官生长发育以及睾丸激素水平、抗氧化能力和免疫水平的影响,为开发和利用当地特色植物资源产品、缓解环境因素导致的应激反应下生殖机能降低和改善海南黑山羊公羔生殖机能提供参考。

1 材料与方法

1.1 试验材料

PSE由中国热带农业科学院热带作物品种资源研究所提供,为假蒟乙醇提取物,其中多酚、黄酮类化合物占比27.5%。采用冷浸法制备,将假蒟整株粉末用95%乙醇浸提、旋转蒸发回收得到假蒟乙醇粗提物,冷冻干燥成粉末状后与沸石粉按体积比1∶1混合均匀,4 ℃保存备用。

1.2 试验设计及饲养管理

试验羊只由中国热带农业科学院热带作物品种资源研究所儋州海南黑山羊养殖基地提供。试验采用单因子完全随机试验设计,选择36只3月龄、体况良好、体重相近的断奶海南黑山羊公羔,随机分为4组,每组9只,单栏饲养。4组试验羊在饲喂基础饲粮的同时分别添加0(CON组)、200(200PSE组)、400(400PSE组)和600 mg/kg PSE(600PSE组)。试验期间基础饲粮的精饲料为玉米-豆粕型,粗饲料为王草,采取精饲料与粗饲料分开饲喂的方法,先精后粗。基础饲粮组成及营养水平见表1。每日08:30和15:00各饲喂1次,自由采食和饮水,每日晨饲前收集和称量昨日剩料量,计算每只试验羊每天的采食量。正试期内,晨饲前用万分之一天平称取每日每只试验羊PSE添加量,放入精料混合后,一次性饲喂给每只试验羊,以保证完全摄入。试验开始前,对单栏进行消毒,对试验羊进行统一驱虫免疫。试验时间为2022年7月至2022年10月,共105 d,其中预试期15 d,正试期90 d。每周按时打扫羊舍,清理粪便并进行环境消毒。每日记录环境温湿度,计算THI指数:THI=0.8×环境温度+(相对湿度/100)×(环境温度-14.4)+46.4[34]。饲养试验结束后,所有试验羊禁食、禁水12 h后进行屠宰,记录宰前活重,采集睾丸和附睾等组织样品,立即取一部分睾丸和附睾等组织样品放置于多聚甲醛中固定,24 h后换75%酒精保存,用于后续组织切片制作;同时另取一部分睾丸组织样品立即置于液氮中,而后-80 ℃冷冻保存,用于试验的后续分析。
表1 基础饲粮组成及营养水平(干物质基础)

Table 1 Composition and nutrient levels of the basal diet (DM basis)%

项目 Items 含量 Content
原料 Ingredients
王草 King grass 50.00
玉米 Corn 34.60
豆粕 Soybean meal 11.00
麦麸 Wheat bran 1.50
食盐 NaCl 0.60
碳酸氢钠 NaHCO3 0.30
预混料 Premix1) 2.00
合计 Total 100.00
营养水平 Nutrient levels2)
总能 GE/(MJ/kg) 17.45
粗蛋白质 CP 13.28
粗脂肪 EE 6.16
中性洗涤纤维 NDF 44.04
酸性洗涤纤维 ADF 19.05
钙 Ca 0.58
磷 P 0.18

1) 预混料为每千克饲粮提供 The premix provided the following per kg of the diet:VA 15 000 IU,VD 5 000 IU,VE 50 mg,Fe 9 mg,Cu 12.5 mg,Zn 100 mg,Mn 130 mg,Se 0.3 mg, I 1.5 mg,Co 0.5 mg。

2) 营养水平均为实测值。All nutrient levels were measured values.

1.3 检测指标及方法

1.3.1 饲粮中营养成分的测定

参照国家或行业标准方法对饲粮中干物质(GB/T 6435—2014)、粗蛋白质(GB/T 6432—2018)、粗脂肪(GB/T 6433—2006)、中性洗涤纤维(GB/T 20806—2006)、酸性洗涤纤维(NY/T 1459—2022)、钙(GB/T 6436—2018)和磷含量(GB/T 6437—2018)进行测定,饲粮中总能使用氧弹量热仪(德国IKA公司,C6000)进行测定。

1.3.2 阴囊、睾丸和附睾发育指标和各级生精细胞密度的测定

分别于正试期的第30天、第60天、第90天测量海南黑山羊阴囊横径、纵径、横围。试验羊屠宰后,记录睾丸重,计算睾丸系数,并测量睾丸的横径、纵径、横围和纵围;记录附睾重,计算附睾系数。生殖器官系数的计算公式为:

睾丸系数或附睾系数=睾丸或附睾重量(g)/宰前活重(kg)。

取睾丸和附睾等组织样品制作的组织切片,用NDP.view软件进行观察,采用五点取样法统计附睾壁厚度、附睾管直径、曲细精管直径和各级生精细胞(间质细胞、支持细胞、精原细胞、精母细胞、精子细胞、精子)密度等数据,取平均值。

1.3.3 睾丸组织中能量代谢酶活性和激素水平的测定

取-80 ℃冷冻保存的睾丸组织测定能量代谢酶活性,具体包括碱性磷酸酶(alkaline phosphatase,AKP)、琥珀酸脱氢酶(succinate dehydrogenase,SDH)、乳酸脱氢酶(lactate dehydrogenase,LDH),测定所用试剂盒购自南京建成生物工程研究所,测定过程严格按照说明书进行。
取-80 ℃冷冻保存的睾丸组织测定激素水平,具体包括皮质酮(corticosterone,CORT)、卵泡刺激素(follicle-stimulating hormone,FSH)、黄体生成素(luteinizing hormone,LH)、睾酮(testosterone,T)、三碘甲状腺原氨酸(triiodothyronine,T3)和四碘甲状腺原氨酸(tetraiodothyronine,T4),测定所用试剂盒购自南京建成生物工程研究所,测定过程严格按照说明书进行。

1.3.4 睾丸组织中抗氧化、免疫和抗热应激指标的测定

取-80 ℃冷冻保存的睾丸组织测定抗氧化指标,具体包括过氧化氢酶(catalase,CAT)、丙二醛(malondialdehyde,MDA)、超氧化物歧化酶(superoxide dismutase,SOD)、谷胱甘肽过氧化物酶(glutathione peroxidase,GSH-Px)、总抗氧化能力(total antioxidant capacity,T-AOC)。
取-80 ℃冷冻保存的睾丸组织测定抗热应激指标,具体包括热休克蛋白27(heat shock protein 27,HSP27)、热休克蛋白70(heat shock protein 70,HSP70)和热休克蛋白90(heat shock protein 90,HSP90)。
取-80 ℃冷冻保存的睾丸组织测定免疫指标,具体包括肿瘤坏死因子-α(tumor necrosis factor-α,TNF-α)、白细胞介素-1β(interleukin-1β,IL-1β)、白细胞介素-2(interleukin-2,IL-2)、白细胞介素-4(interleukin-4,IL-4)、白细胞介素-6(interleukin-6,IL-6)、免疫球蛋白A(immunoglobulin A,IgA)、免疫球蛋白G(immunoglobulin G,IgG)、免疫球蛋白M(immunoglobulin M,IgM)。
上述指标测定所用试剂盒均购自南京建成生物工程研究所,测定过程严格按照说明书进行。

1.4 统计分析

应用Excel 2019对试验数据进行初步整理,使用SPSS 25.0统计软件进行方差分析和显著性检验,采用one-way ANOVA中的Duncan氏法进行多重比较,并进行线性和二次回归分析,结果用平均值和均值标准误(SEM)表示,以P<0.05表示差异显著,0.05≤P<0.10表示有趋势。

2 结果与分析

2.1 试验期间采食量和THI变化

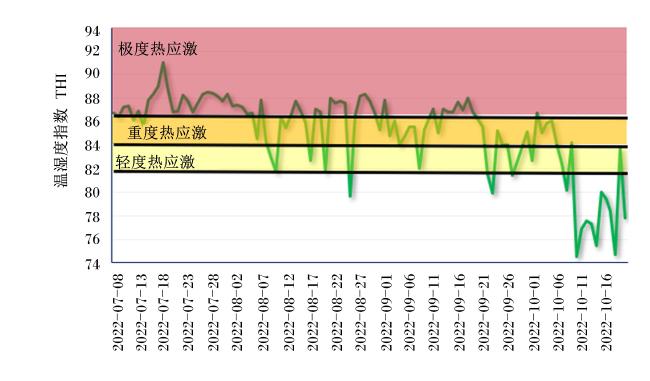
表2可知,饲粮中添加不同水平PSE对海南黑山羊日干物质采食量无显著影响(P>0.05)。本试验开展时间为2022年7月8日至2022年10月20日,试验期间海南省处于夏季,环境高温、高湿,羊舍THI变化如图1所示,THI≥82的天数占试验全期的86.67%,表明试验动物处于热应激环境中。
表2 假蒟提取物对海南黑山羊日干物质采食量的影响

Table 2 Effects of PSE on daily dry matter feed intake of Hainan black goatsg/d

项目
Item
组别 Groups SEM PP-value
CON 200PSE 400PSE 600PSE 处理
Treatment
线性
Linear
二次
Quadratic
日干物质采食量
Daily dry matter feed intake
387.93 386.81 390.28 374.09 8.819 0.924 0.645 0.684

同行数据肩标不同小写字母表示差异显著(P<0.05),相同或无字母表示差异不显著(P>0.05)。下表同。

In the same row, values with different small letter superscripts mean significant difference (P<0.05), while with the same or no letter superscripts mean no significant difference (P>0.05). The same as below.

图1 试验期间羊舍THI变化

Fig.1 THI change in goat house during experimental period

2.2 PSE对海南黑山羊阴囊、睾丸和附睾生长发育的影响

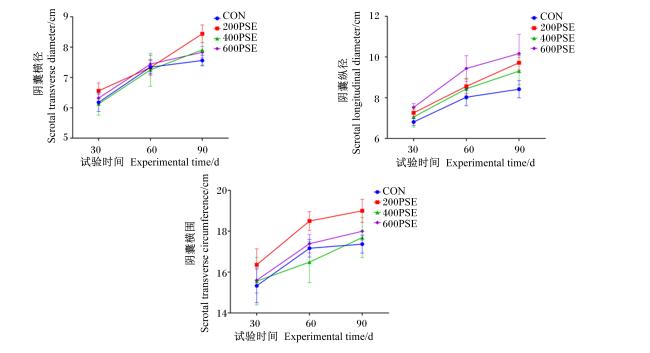
图2可知,与CON组比较,饲粮中添加不同水平PSE时海南黑山羊阴囊横径、纵径以及横围都有所提高,其中横径在添加量为200 mg/kg时达到最高,比CON组提高18.06%;纵径在添加量为600 mg/kg时达到最高,比CON组提高23.15%;而横围在添加量为200 mg/kg时达到最高,比CON组提高20.34%。但方差分析结果显示,饲粮中添加不同水平PSE对海南黑山羊阴囊各发育指标均无显著影响(P>0.05)。
图2 假蒟提取物对海南黑山羊阴囊生长发育的影响

CON:CON组 CON group;200PSE:200PSE组 200PSE group;400PSE:400PSE组 400PSE group;600PSE:600PSE组 600PSE group。下图同 the same as below。

Fig.2 Effects of PSE on scrotal growth and development of Hainan black goats

表3可知,饲粮中添加不同水平PSE对海南黑山羊睾丸重、睾丸横径、睾丸纵径、睾丸横围、睾丸纵围、睾丸系数、附睾重和附睾系数的影响均不显著(P>0.05)。与CON组相比,饲粮中添加200、400、600 mg/kg PSE使睾丸重分别提高了10.73%、4.26%、8.58%,使附睾重分别提高了24.82%、36.04%、32.46%。
表3 假蒟提取物对海南黑山羊睾丸和附睾生长发育的影响

Table 3 Effects of PSE on testicular and epididymal growth and development of Hainan black goats

项目
Items
组别 Groups SEM PP-value
CON 200PSE 400PSE 600PSE 处理
Treatment
线性
Linear
二次
Quadratic
宰前活重
Live weight before slaughter/kg
13.19 13.66 14.29 13.29 0.298 0.573 0.733 0.235
睾丸重
Testis weight/g
98.44 109.00 102.63 106.89 3.862 0.785 0.594 0.696
睾丸系数
Testis index/(g/kg)
8.28 8.51 8.56 8.32 0.206 0.952 0.918 0.569
睾丸横径
Testis transverse diameter/cm
5.61 5.31 5.14 5.44 0.079 0.222 0.333 0.063
睾丸纵径
Testis longitudinal diameter/cm
9.27 9.92 8.57 10.02 0.220 0.084 0.616 0.346
睾丸横围
Testis transverse circumference/cm
11.22 11.44 11.36 11.39 0.144 0.957 0.756 0.755
睾丸纵围
Testis longitudinal circumference/cm
17.67 17.78 17.93 18.06 0.284 0.967 0.616 0.989
附睾重
Epididymis weight/g
4.19 5.23 5.70 5.55 0.360 0.559 0.163 0.420
附睾系数
Epididymis index/(g/kg)
0.35 0.40 0.42 0.43 0.024 0.638 0.228 0.655

2.3 PSE对海南黑山羊睾丸和附睾组织结构的影响

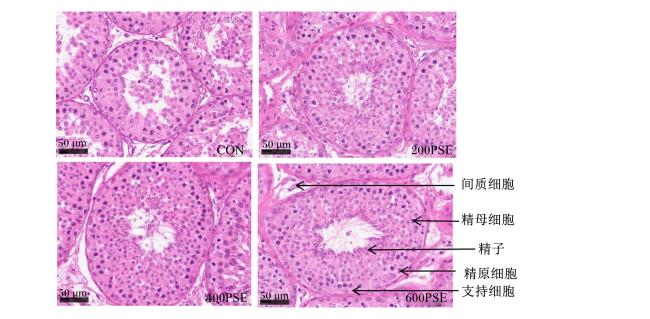
图3可知,与添加PSE的3个试验组相比,CON组各级生精细胞数目较少,排列紊乱,甚至没有精子,已出现细胞凋亡现象(未成熟的细胞掉落至管腔中);曲细精管空腔化更为严重。3个试验组的各级生精细胞数目均明显高于对照组,且排列紧密,管腔面可见发育成熟的精子。此外,400PSE组各级生精细胞数目明显高于其他试验组。由表4可知,400PSE组和600PSE组曲细精管直径显著大于CON组和200PSE组(P<0.05);饲粮中添加不同水平PSE对曲细精管间质细胞、支持细胞、精原细胞、精母细胞、精子细胞和精子密度均有不同程度的提高作用,除了间质细胞外的其他生精细胞的密度均在PSE添加量为400 mg/kg时最高,且显著高于CON组(P<0.05)。
图3 假蒟提取物对海南黑山羊睾丸组织形态学的影响

Fig.3 Effects of PSE on histomorphology of testis of Hainan black goats (400×)

表4 假蒟提取物对海南黑山羊睾丸中各级生精细胞密度的影响

Table 4 Effects of PSE on spermatogonial cell density at all levels in testis of Hainan black goats

项目
Items
组别 Groups SEM PP-value
CON 200PSE 400PSE 600PSE 处理
Treatment
线性
Linear
二次
Quadratic
曲细精管直径
Seminiferous tubule diameter/μm
188.41b 191.52b 198.70a 200.98a 1.085 <0.001 <0.001 0.747
各级生精细胞密度 Spermatogonial cell density at all levels/(个/mm2)
间质细胞 Interstitial cells 16.75 17.56 18.00 18.50 0.421 0.538 0.151 0.859
支持细胞 Sertoli cells 90.63b 93.67b 102.88a 85.63b 1.749 0.002 0.659 0.001
精原细胞 Spermatogonia 174.63b 195.11a 205.13a 181.00b 2.961 <0.001 0.156 <0.001
精母细胞 Spermatocyte 207.75b 248.33a 269.25a 208.63b 5.796 <0.001 0.487 <0.001
精子细胞 Sperm cells 340.00b 391.78a 405.63a 401.88a 6.470 <0.001 <0.001 0.010
精子 Sperm 95.75b 113.78a 113.75a 100.13ab 2.937 0.048 0.596 0.007
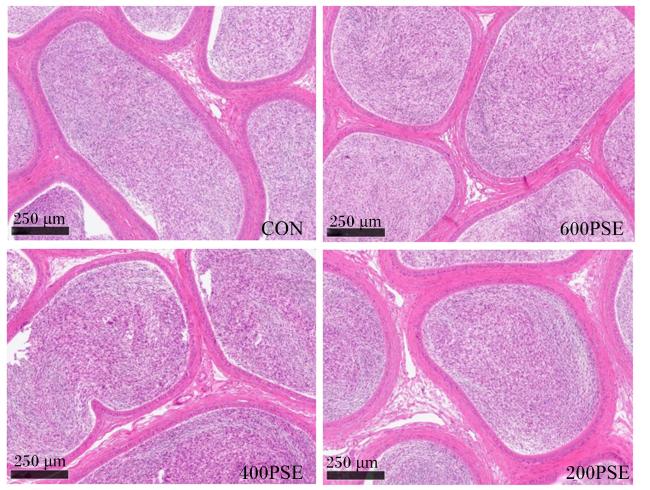
图4可知,3个试验组的附睾壁较CON组薄,附睾管直径从图中并看不出明显区别。由表5可知,3个试验组附睾管壁厚度有低于CON组的趋势(P=0.089),附睾管直径高于CON组,但无显著差异(P>0.05)。
图4 假蒟提取物对海南黑山羊附睾组织形态学的影响

Fig.4 Effects of PSE on histomorphology of epididymis of Hainan black goats (50×)

表5 假蒟提取物对海南黑山羊附睾组织结构的影响

Table 5 Effects of PSE on histological structure of epididymis of Hainan black goatsμm

项目
Items
组别 Groups SEM PP-value
CON 200PSE 400PSE 600PSE 处理
Treatment
线性
Linear
二次
Quadratic
附睾管直径
Epididymal canal diameter
447.61 457.14 477.03 467.91 7.225 0.533 0.222 0.530
附睾管壁厚度
Epididymal wall thickness
61.23 58.41 55.00 52.97 1.383 0.089 0.023 0.884

2.4 PSE对海南黑山羊睾丸组织中能量代谢酶活性和激素水平的影响

表6可知,与CON组相比,400PSE组睾丸组织中SDH活性显著增加(P<0.05);睾丸组织中AKP和LDH活性各组之间无显著差异(P>0.05)。由表7可知,饲粮中添加不同水平PSE对睾丸组织中T和LH水平产生了显著影响(P<0.05),400PSE组较600PSE组显著降低(P<0.05)。饲粮中添加不同水平PSE对海南黑山羊睾丸组织中T3、T4、FSH、CORT水平无显著影响(P>0.05)。
表6 假蒟提取物对海南黑山羊睾丸组织中能量代谢酶活性的影响

Table 6 Effects of PSE on growth energy metabolism enzyme activities in testicular tissue of Hainan black goats

项目
Items
组别 Groups SEM PP-value
CON 200PSE 400PSE 600PSE 处理
Treatment
线性
Linear
二次
Quadratic
碱性磷酸酶
AKP/(金氏单位/g prot)
38.26 40.46 34.26 41.68 1.053 0.068 0.642 0.196
琥珀酸脱氢酶 SDH/(U/mg prot) 8.20b 8.76ab 9.76a 7.79b 0.229 0.013 0.903 0.004
乳酸脱氢酶 LDH/(U/g prot) 2 362.30 2 378.71 2 436.79 2 527.58 38.857 0.456 0.128 0.646
表7 假蒟提取物对海南黑山羊睾丸组织中激素水平的影响

Table 7 Effects of PSE on hormone levels in testicular tissue of Hainan black goatsng/mg prot

项目
Items
组别 Groups SEM PP-value
CON 200PSE 400PSE 600PSE 处理
Treatment
线性
Linear
二次
Quadratic
睾酮 T 0.52ab 0.53ab 0.45b 0.56a 0.013 0.040 0.558 0.058
三碘甲状腺原氨酸 T3 0.97 1.01 0.89 1.05 0.022 0.066 0.563 0.162
四碘甲状腺原氨酸 T4 25.08 27.63 25.07 26.79 0.445 0.097 0.496 0.629
黄体生成素 LH 1.02ab 1.07ab 0.90b 1.12a 0.026 0.001 0.578 0.075
卵泡刺激素 FSH 0.85 0.91 0.82 0.91 0.016 0.129 0.455 0.657
皮质醇 CORT 7.42 7.99 7.55 8.10 0.140 0.244 0.196 0.968

2.5 PSE对海南黑山羊睾丸组织中抗氧化、免疫和抗热应激指标的影响

表8可知,饲粮中添加不同水平PSE后海南黑山羊睾丸组织中T-AOC有不同程度提高,其中400PSE组和600PSE组与CON组的差异达到显著水平(P<0.05),分别较CON组提高了13.08%、7.69%;此外,饲粮中PSE添加量对睾丸组织中T-AOC具有线性和二次效应(P<0.05)。饲粮中添加不同水平PSE显著提高了睾丸组织中SOD活性(P<0.05),并有提高CAT活性的趋势(P=0.052)。与CON组相比,200PSE组、400PSE组和600PSE组睾丸组织中SOD活性分别提高了14.11%、23.45%、17.20%;此外,饲粮中PSE添加量对睾丸组织中SOD活性具有线性和二次效应(P<0.05)。睾丸组织中GSH-Px活性和MDA含量各组之间均无显著差异(P>0.05)。
表8 假蒟提取物对海南黑山羊睾丸组织中抗氧化指标的影响

Table 8 Effects of PSE on antioxidant indices in testicular tissue of Hainan black goats

项目
Items
组别 Groups SEM PP-value
CON 200PSE 400PSE 600PSE 处理
Treatment
线性
Linear
二次
Quadratic
总抗氧化能力
T-AOC/(U/mg prot)
1.30c 1.34bc 1.47ab 1.40a 0.017 0.001 0.002 0.067
丙二醛 MDA/(nmol/mg prot) 1.73 1.68 1.65 1.51 0.090 0.852 0.405 0.822
过氧化氢酶 CAT/(U/mg prot) 4.33 4.85 4.92 5.57 0.169 0.052 0.011 0.834
谷胱甘肽过氧化物酶
GSH-Px/(U/mg prot)
36.71 39.10 35.83 33.69 0.965 0.252 0.151 0.242
超氧化物歧化酶
SOD/(U/mg prot)
57.27b 65.35a 70.70a 67.12a 1.515 0.009 0.005 0.035
表9可知,饲粮中PSE添加量对睾丸组织中IgG含量有显著影响(P<0.05),且具有线性效应(P<0.05)。与CON组相比,200PSE组、400PSE组和600PSE组睾丸组织中IgG含量分别提高了9.73%(P<0.05)、4.18%(P>0.05)、10.83%(P<0.05)。睾丸组织中抗炎因子IL-4含量在CON组最低,200PSE组、400PSE组和600PSE组相对于CON组分别提高了7.56%(P>0.05)、2.66%(P>0.05)、15.46%(P<0.05)。
表9 假蒟提取物对海南黑山羊睾丸组织中免疫指标的影响

Table 9 Effects of PSE on immune indices in testicular tissue of Hainan black goats

项目
Items
组别 Groups SEM PP-value
CON 200PSE 400PSE 600PSE 处理
Treatment
线性
Linear
二次
Quadratic
免疫球蛋白A IgA/(μg/mg prot) 32.08 34.36 31.68 33.81 0.607 0.343 0.639 0.950
免疫球蛋白G IgG/(μg/mg prot) 47.36b 51.97a 49.34ab 52.49a 0.761 0.048 0.049 0.606
免疫球蛋白M IgM/(μg/mg prot) 20.67 21.58 19.59 22.66 0.428 0.071 0.274 0.188
白细胞介素-6 IL-6/(ng/g prot) 17.66 19.10 17.41 18.47 0.393 0.428 0.834 0.816
白细胞介素-4 IL-4/(ng/g prot) 11.64b 12.52ab 11.95b 13.44a 0.243 0.037 0.020 0.491
白细胞介素-2 IL-2/(ng/g prot) 5.89 6.17 5.70 6.62 0.144 0.121 0.167 0.260
白细胞介素-1β
IL-1β/(ng/g prot)
4.50 4.64 4.28 4.76 0.097 0.362 0.623 0.371
肿瘤坏死因子-α
TNF-α/(ng/g prot)
16.52 16.44 14.84 17.61 0.377 0.079 0.599 0.054
表10可知,与CON组相比,当PSE添加量为600 mg/kg时,海南黑山羊睾丸组织中HSP27含量显著提高了10.77%(P<0.05);睾丸组织中HSP90和HSP70含量各组之间均无显著差异(P>0.05)。
表10 假蒟提取物对海南黑山羊睾丸组织中抗热应激指标的影响

Table 10 Effects of PSE on anti-heat stress indices in testicular tissue of Hainan black goatsng/mg prot

项目
Items
组别 Groups SEM PP-value
CON 200PSE 400PSE 600PSE 处理
Treatment
线性
Linear
二次
Quadratic
热休克蛋白90 HSP90 4.47 4.77 4.61 4.77 0.087 0.556 0.345 0.670
热休克蛋白70 HSP70 0.81 0.87 0.82 0.86 0.015 0.487 0.446 0.917
热休克蛋白27 HSP27 0.65b 0.70ab 0.64b 0.72a 0.012 0.040 0.096 0.444

3 讨论

3.1 PSE对海南黑山羊阴囊、睾丸和附睾生长发育的影响

评估动物机体遭受热应激有多个参数,例如外界环境温湿度、THI、直肠温度、呼吸速率、深度和频率、血液生化指标和热休克蛋白含量等,而THI是评估家畜是否存在热应激及热应激程度的最常用指标。本试验于7—10月份在海南省儋州市开展,此时正值该地区典型的夏季,气候特点高温、高湿。基于前人对山羊THI的界定,THI被划分为4个等级:无热应激(THI<82)、轻度热应激(82≤THI<84)、重度热应激(84≤THI<86)以及极重度热应激(THI≥86)[35],这一分类为本研究提供了科学的评价基准。本研究对海南黑山羊的热应激状态进行了详尽的量化分析,THI平均值范围在75~91,这表明所有试验羊在整个试验期都处于热应激状态下,个别时期处于严重的热应激状态。热应激作为外部影响雄性生殖过程的一个重要的环境因素,直接影响哺乳动物可活动和生育的精子生成过程[36]。热应激会导致睾丸组织和细胞损伤,造成精子发生异常。天然植物提取物含有多种活性成分,如黄酮、生物碱和多酚等,可以通过清除体内的自由基减少氧化损伤,进而保护睾丸组织的结构和功能。本研究中的试验材料PSE主要是由多种活性成分组成的混合物,其主要成分为多酚、黄酮类化合物(27.5%)。本试验结果表明,饲粮中添加PSE可提高夏季海南黑山羊睾丸重,并有提高睾丸纵径的趋势,说明PSE的添加可以在一定程度上促进睾丸的生长和发育。在整个夏季饲养阶段,饲粮中添加PSE对海南黑山羊阴囊的生长发育无不良影响。在本试验条件下通过睾丸组织切片观察到,3个试验组睾丸发育较好于CON组。这表明在整个饲养试验阶段,饲粮中添加PSE能够改善热应激条件下海南黑山羊生殖器官发育状态,并对生殖细胞发育有益。睾丸发育过程与精子生成过程密切相关。精子的产生取决于睾丸结构的正常发育,其中包括支持细胞、间质细胞和生殖细胞在各个阶段的生长和分化。本研究结果显示,在饲粮中添加不同水平的PSE均提高了支持细胞的密度,进而提高精原细胞以及精子细胞的密度,同时成熟精子密度也增多,且以PSE添加量为400 mg/kg时效果最好。上述结果表明,PSE可能通过保护热应激条件下海南黑山羊睾丸的正常发育来使精子发生进程正常有序进行,这可能得益于PSE中抗氧化活性物质如黄酮、多酚和生物碱类等发挥了作用,保护睾丸组织免受高温、高湿的热应激环境导致的氧化损伤。

3.2 PSE对海南黑山羊睾丸组织中能量代谢酶活性和激素水平的影响

AKP、SDH和LDH在睾丸发育和成熟过程中起着关键作用。睾丸组织中AKP的表达水平随着发育和成熟而发生变化,其活性在青春期和性成熟期间显著增加。AKP存在于睾丸生殖细胞系中,如精原细胞和精子细胞,其活性与精子的发育和成熟密切相关[37]。睾丸作为能量消耗较大的组织,其正常的能量代谢对于维持精子生成和生殖功能至关重要。SDH的活性可直接影响睾丸组织的能量供应,SDH还参与调节睾丸组织中的氧化应激反应。氧化应激是由于细胞内产生的自由基或活性氧物质超过细胞抗氧化能力而导致的一种生物学反应。在睾丸组织中,SDH的活性可以影响线粒体功能和活性氧物质的产生,从而调节睾丸细胞的氧化应激水平[38]。在睾丸组织中,LDH的活性影响了细胞内乳酸的生成和转化。睾丸能量消耗较大,需要大量的ATP来支持精子的发生和生殖功能。LDH在睾丸组织中调节了糖酵解途径,使得细胞可以通过乳酸发酵产生ATP,从而维持睾丸细胞的正常能量代谢[39]。本试验条件下,饲粮中添加PSE对夏季热应激状态下海南黑山羊公羔睾丸组织中AKP和LDH活性无显著影响,但在PSE添加量为400 mg/kg时睾丸组织中SDH活性显著提高,这可能是400PSE组的睾丸精原细胞以及精细胞、精子数目等增多的原因,进而促进了睾丸的发育,但在PSE添加量为600 mg/kg时又出现下降,其中变化的机制还有待进一步研究。
有大量的研究证明了雄性动物的繁殖能力与下丘脑-垂体-性腺和下丘脑-垂体-肾上腺轴密切相关[40-42]。生殖细胞数量和精子发生取决于通过支持细胞分泌的FSH和T的作用[43-44]。FSH在生育能力中起着至关重要的作用,因为它影响围产期和初情期期间支持细胞的增殖,促进生殖细胞与睾丸发育所需支持细胞衍生因子产生[45]。T对睾丸中精子发生、支持细胞增殖和间质细胞发育以及附睾发育至关重要,其与支持细胞合成的雄激素结合蛋白以及支持细胞、间质细胞和肾小管周围细胞中的雄激素受体结合促进睾丸与附睾的生长发育。T和FSH通过睾丸支持细胞的协同作用调节雄性繁殖能力,FSH通过支持细胞上的受体刺激精子发生[46]。LH可加速睾丸间质细胞中T的产生,从而影响支持细胞来促进精子发生[47]。LH以内分泌的方式发挥作用,负反馈调节FSH的分泌。在睾丸中,LH与FSH结合以触发支持细胞增殖和生殖细胞分化,并且FSH也受LH和起抑制作用的旁分泌模式的调节[48]。本研究结果显示,以600PSE组海南黑山羊睾丸组织中T和LH的水平最高。生殖激素的调控途径复杂而多样,受负反馈调节影响等,LH、FSH作用于睾丸间质细胞,促进T的生成,FSH水平在200PSE组、600PSE组略有上升,导致T水平也上升,从而有利于精子的发生,而400PSE组通过切片观察可以看到各级生精细胞发育最好,这表明可能已经受到生殖激素负反馈调节的影响。
甲状腺特别容易受到环境温度波动的影响,其在调节新陈代谢活动和重要的细胞功能(如耗氧量和产热量)方面发挥着关键作用。研究表明,甲状腺激素T3与T4的核心作用在于提高新陈代谢,促进葡萄糖供给细胞,有利于免疫球蛋白生成与脂肪分解,有益于保护肝脏与脑神经系统[45]。夏季热应激对动物机体造成的损害通常可以通过机体进行适度调节,主要是减少甲状腺激素向机体的释放和使动物的基础代谢削弱来缓解;而在热应激反应的过程中,CORT作为热应激反应标志物,其水平的变化反映动物所受热应激程度。CORT主要功能包括促进蛋白质分解为氨基酸供能、促进非糖物质转化为葡萄糖以应对应激状况下的能量需求[49]。而在本试验条件下,饲粮中添加不同水平PSE后海南黑山羊睾丸组织中CORT水平并无明显变化,在一定程度说明PSE起到了缓解热应激的作用。有研究发现,增加羊舍通风强度可提高9周龄羔羊体内甲状腺激素水平[47]。对比冷应激环境,绵羊在夏季热应激下血清T3与T4水平显著升高,揭示热应激状态下甲状腺激素分泌显著增强[50]。本试验中,3个试验组海南黑山羊睾丸组织中T4水平增加,且以200PSE组最高,T3水平则在200PSE组、600PSE组略有上升,说明PSE有缓解海南黑山羊公羔夏季热应激的功效。

3.3 PSE对海南黑山羊睾丸组织中抗氧化、免疫和抗热应激指标的影响

雄性动物的精子发生过程容易受外界环境温度影响,若对温度极其敏感的睾丸受到热应激,则会产生大量自由基,从而使睾丸受到氧化损伤[51]。不平衡的氧化-抗氧化状态会导致细胞中活性氧和含氮自由基的积累,从而破坏蛋白质、脂类、DNA和RNA的结构,影响其正常功能[52-53]。热应激影响雄性生殖性能的另外一种作用方式是物理作用方式,夏季热应激会使畜体散热不畅,阴囊和睾丸温度持续升高,热调节能力失去作用[50],致使精浆蛋白[54]、抗氧化酶[55]、热休克蛋白[56]发生变化,上述变化会使机体中自由基不能被及时有效清除而发生积累,发生氧化应激[57-58],进而阻碍睾丸的生精功能。
睾丸和精浆中丰富的抗氧化酶系统以及非酶抗氧化剂共同构成了一道防线,以维持氧化应激与抗氧化剂之间的动态平衡。CAT和GSH-Px等抗氧化酶在一系列信号转导的刺激下,可直接或间接清除活性氧自由基,从而消除氧化应激的有害影响[59],这些物质可保护细胞和生物体免受活性氧自由基造成的氧化应激[60]。MDA是脂质过氧化的最终产物,可以反映脂质氧化的程度[61],T-AOC是抗氧化酶和其他抗氧化物质的综合水平,与整体健康密切相关,GSH-Px在雄性动物生殖系统的抗氧化机制中占据核心地位,尤其在睾丸和精子发生初期,其高度表达为精子发生提供了必要的抗氧化保护,对精子发生过程至关重要[58,62]。已有研究揭示,当山羊经历8 h急性夏季高温暴露时,其血清中T-AOC、SOD和GSH-Px的活性均呈现出下降趋势,而脂质过氧化产物MDA的含量在短短4 h内便迅速升高[56]。Shamsi等[63]研究进一步证实精浆内MDA含量的升高与精子形态异常及DNA损伤风险的增加有直接关系。本试验结果表明,饲粮中添加PSE提高了海南黑山羊睾丸组织中SOD活性和T-AOC,并且有提高CAT活性的趋势。前人的研究结果表明,饲粮中添加PSE显著提高了海南黑山羊血清中SOD活性和T-AOC[64]。这表明PSE可以改善夏季热应激状态下海南黑山羊睾丸组织的抗氧化能力,这可能得益于PSE中如黄酮类、多酚和生物碱等能够发挥抗氧化能力的生物活性物质。
此外,天然植物提取物不仅具有抗氧化活性,还具有免疫调节能力。动物机体的免疫能力主要取决于细胞因子和免疫球蛋白。白细胞介素(IL)等细胞因子是使免疫系统细胞之间进行交流以产生免疫反应的分子信使,而活化的B细胞产生的免疫球蛋白可保护宿主免受细胞外病原体的侵害[65]。在体液免疫中发挥主要作用的免疫物质是血清免疫球蛋白,IgG、IgM和IgA是其主要的组成部分,发挥免疫功能的途径是清除病原体,并主要通过测定免疫球蛋白含量高低的方式来反映机体当前的免疫功能。细胞因子是免疫细胞制造和释放的小分子肽类,它们在调节免疫系统方面发挥着重要作用,包括白细胞介素、肿瘤坏死因子超家族、干扰素和趋化因子等,并且这些因子可分为两类:促炎因子(如IL-1β和IL-α等)和抗炎因子(如IL-2和IL-4等)[66],其中促炎性白细胞介素可促进炎症反应,从而增强免疫反应,加速清除体内病原体;而抗炎性白细胞介素则直接抑制炎症反应。研究显示,假蒟可以有效抑制炎性因子的分泌,具有较强的抗炎活性[67]。Wang等[68]以21日龄仔猪作为动物模型,连续14 d在饲粮中添加PSE,在添加量为50 mg/kg时观察到血清中IL-1β、IL-6及TNF-α等炎性因子的含量显著降低,表明其在调控炎性反应方面具有积极作用,并推断PSE中的生物碱和酚类成分可能是其抗炎效应的关键来源。在21日龄断奶仔猪饲粮中添加不同水平PSE,可以显著提高断奶仔猪血液中血小板的数量,增加相关免疫球蛋白(包括IgG、IgM和IgA)的含量。本试验结果显示,在饲喂添加不同水平PSE的饲粮后,海南黑山羊睾丸组织中IgG、IgM以及IL-4的含量都有不同程度的上升,说明PSE可以通过促进免疫球蛋白和抗炎因子的分泌,从而提高睾丸组织的免疫水平。其原因可能是PSE中含有的生物碱和酚类物质等活性物质提高了机体内抗炎因子的释放和减少了机体的炎症反应,从而达到提高机体免疫功能的作用。
热休克蛋白(HSP)是一种保守的蛋白质,也称为“分子伴侣”,参与有助于保护细胞和细胞成分免受环境波动的途径[69]。在热应激下,可观察到的HSP是HSP110、HSP100、HSP90、HSP70、HSP60、HSP40、HSP10和其他小分子蛋白家族[70]。HSP60具有促凋亡的作用,而HSP70、HSP90和HSP27主要起抗凋亡的作用[71]。它们在防止蛋白质降解方面很重要,并且在非活性形式的蛋白质的细胞内转运中起着至关重要的作用[72]。本试验中,600PSE组中HSP27含量较CON组显著增加,HSP90、HSP70含量也高于CON组,但影响有限,说明在饲粮中添加PSE可以促进于公羔生殖器官睾丸组织中HSP的生成,更好地帮助机体抵御夏季热应激带来的负面影响,具体机制还有待进一步研究。

4 结论

饲粮中添加PSE可提高夏季热应激状态下海南黑山羊睾丸组织中SOD活性和T-AOC,并可提高睾丸组织中抗炎因子IL-4和热休克蛋白HSP27含量以及SDH活性和LH水平,改善睾丸组织的抗氧化能力和免疫水平以及能量代谢,从而有助于缓解夏季热应激引起的氧化损伤,促进海南黑山羊公羔生殖器官的生长和发育,且在添加量为400 mg/kg时效果较好。
[1]
FULLER A, MITCHELL D, MALONEY S K, et al. How dryland mammals will respond to climate change: the effects of body size, heat load and a lack of food and water[J]. Journal of Experimental Biology, 2021, 224(Suppl.1):jeb238113.

[2]
RENAUDEAU D, COLLIN A, YAHAV S, et al. Adaptation to hot climate and strategies to alleviate heat stress in livestock production[J]. Animal:an International Journal of Animal Bioscience, 2012, 6(5):707-728.

[3]
NARDONE A, RONCHI B, LACETERA N, et al. Effects of climate changes on animal production and sustainability of livestock systems[J]. Livestock Science, 2010, 130(1/2/3):57-69.

[4]
SEJIAN V, BHATTA R, GAUGHAN J B, et al. Review:adaptation of animals to heat stress[J]. Animal, 2018, 12(Suppl.2):S431-S444.

[5]
BOHMANOVA J, MISZTAL I, COLE J B. Temperature-humidity indices as indicators of milk production losses due to heat stress[J]. Journal of Dairy Science, 2007, 90(4):1947-1956.

PMID

[6]
FUQUAY J W. Heat stress as it affects animal production[J]. Journal of Animal Science, 1981, 52(1):164-174.

DOI PMID

[7]
LIU A N, LI L Q, CHEN X L, et al. Effects of heat stress on body temperature,milk production,and reproduction in dairy cows: a novel idea for monitoring and evaluation of heat stress—a review[J]. Asian-Australasian Journal of Animal Sciences, 2019, 32(9):1332-1339.

[8]
GONZALEZ-RIVAS P A, CHAUHAN S S, HA M, et al. Effects of heat stress on animal physiology,metabolism,and meat quality:a review[J]. Meat Science, 2020,162:108025.

[9]
CUI Y J, GU X H. Proteomic changes of the porcine small intestine in response to chronic heat stress[J]. Journal of Molecular Endocrinology, 2015, 55(3):277-293.

DOI PMID

[10]
HASHEM M, HOSSAIN M, RANA M, et al. Effect of heat stress on blood parameter,carcass and meat quality of black Bengal goat[J]. Bangladesh Journal of Animal Science, 2013, 42(1):57-61.

[11]
PRAGNA P, SEJIAN V, BAGATH M, et al. Comparative assessment of growth performance of three different indigenous goat breeds exposed to summer heat stress[J]. Journal of Animal Physiology and Animal Nutrition, 2018, 102(4):825-836.

DOI PMID

[12]
SALAMA A, CAJA G, HAMZAOUI S, et al. Different levels of response to heat stress in dairy goats[J]. Small Ruminant Research, 2014, 121(1):73-79.

[13]
RATO L, ALVES M G, SOCORRO S, et al. Metabolic regulation is important for spermatogenesis[J]. Nature Reviews Urology, 2012, 9(6):330-338.

DOI PMID

[14]
MIEUSSET R, BUJAN L. Testicular heating and its possible contributions to male infertility:a review[J]. International Journal of Andrology, 1995, 18(4):169-184.

[15]
HARRISON R G, WEINER J S. Vascular patterns of the mammalian testis and their functional significance[J]. Journal of Experimental Biology, 1949, 26(3):304-316.

PMID

[16]
NGOULA F, LONTIO F A, TCHOFFO H, et al. Heat induces oxidative stress:reproductive organ weights and serum metabolite profile,testes structure,and function impairment in male cavy (Cavia porcellus)[J]. Frontiers in Veterinary Science, 2020,7:37.

[17]
WANG K, LI Z J, LI Y S, et al. Impacts of elevated temperature on morphology,oxidative stress levels,and testosterone synthesis in ex vivo cultured porcine testicular tissue[J]. Theriogenology, 2023,212:181-188.

[18]
刘蕴蝶. 褪黑素对夏季高温所致的奶山羊精液质量低下的保护作用研究[D]. 硕士学位论文. 杨凌: 西北农林科技大学, 2023.

LIU Y D. Study on the protective effect of melatonin on low semen quality in dairy goats due to the high temperatures in summer[D]. Master’s Thesis. Yangling: Northwest A&F University, 2023. (in Chinese)

[19]
CONG X, ZHANG Q, LI H T, et al. Puerarin ameliorates heat stress-induced oxidative damage and apoptosis in bovine Sertoli cells by suppressing ROS production and upregulating Hsp72 expression[J]. Theriogenology, 2017,88:215-227.

[20]
WEI C, LI J, MA Z, et al. Study on the best extraction technology of total flavonoids from Piper sarmentosum Roxb. leaves and evaluation of antioxidant activity[J]. IOP Conference Series:Earth and Environmental Science, 2019, 330(4):042061.

[21]
MATHEW S P, MOHANDAS A, NAIR G. Piper sarmentosum Roxb.—an addition to the flora of Andaman islands[J]. Current Science, 2004, 87(2):141-142.

[22]
YEO E, WONG K, SEE M L, et al. Piper sarmentosum Roxb. confers neuroprotection on beta-amyloid(Aβ)-induced microglia-mediated neuroinflammation and attenuates tau hyperphosphorylation in SH-SY5Y cells[J]. Journal of Ethnopharmacology, 2018,217:187-194.

[23]
MD SALLEH M F R R, AMINUDDIN A, HAMID A A, et al. Piper sarmentosum Roxb. attenuates vascular endothelial dysfunction in nicotine-induced rats[J]. Frontiers in Pharmacology, 2021,12:667102.

[24]
SUN X L, CHEN W H, DAI W, et al. Piper sarmentosum Roxb.:a review on its botany,traditional uses,phytochemistry,and pharmacological activities[J]. Journal of Ethnopharmacology, 2020,263:112897.

[25]
AKMAL M N, ABDEL AZIZ I, NUR AZLINA M F. Piper sarmentosum Roxb. methanolic extract prevents stress-induced gastric ulcer by modulating oxidative stress and inflammation[J]. Frontiers in Pharmacology, 2022,13:971443.

[26]
AMRAN A A, ZAKARIA Z, OTHMAN F, et al. Aqueous extract of piper sarmentosum decreases atherosclerotic lesions in high cholesterolemic experimental rabbits[J]. Lipids in Health and Disease, 2010,9:44.

[27]
ZAKARIA Z A, PATAHUDDIN H, MOHAMAD A S, et al. In vivo anti-nociceptive and anti-inflammatory activities of the aqueous extract of the leaves of piper sarmentosum[J]. Journal of Ethnopharmacology, 2010, 128(1):42-48.

[28]
MAKCHUCHIT S, RATTAROM R, ITHARAT A. The anti-allergic and anti-inflammatory effects of Benjakul extract (a Thai traditional medicine),its constituent plants and its some pure constituents using in vitro experiments[J]. Biomedicine & Pharmacotherapy, 2017,89:1018-1026.

[29]
WANG D F, ZHOU L L, ZHOU H L, et al. Chemical composition and anti-inflammatory activity of n-butanol extract of Piper sarmentosum Roxb. in the intestinal porcine epithelial cells (IPEC-J2)[J]. Journal of Ethnopharmacology, 2021,269:113723.

[30]
陈川威, 周璐丽, 王定发, 等. 假蒟提取物的体外抗氧化和抗炎效果研究[J]. 中国畜牧兽医, 2019, 46(3):677-683.

DOI

CHEN C W, ZHOU L L, WANG D F, et al. Study on antioxidant and anti-inflammatory effects of extracts from Piper sarmentosum Roxb. in vitro[J]. China Animal Husbandry & Veterinary Medicine, 2019, 46(3):677-683. (in Chinese)

[31]
王定发, 周璐丽, 周雄, 等. 假蒟提取物对断奶仔猪生长性能、血液指标的影响[J]. 动物营养学报, 2015, 27(10):3233-3240.

WANG D F, ZHOU L L, ZHOU X, et al. Effects of Piper sarmentosum extracts on growth performance and blood indexes of weaned piglets[J]. Chinese Journal of Animal Nutrition, 2015, 27(10):3233-3240. (in Chinese)

[32]
王定发, 周璐丽, 周汉林. 假蒟提取物对文昌鸡生长性能、屠宰性能和肉品质的影响[J]. 家畜生态学报, 2017, 38(10):33-37.

WANG D F, ZHOU L L, ZHOU H L. Effects of Piper sarmentosum extract on the growth performance, carcass characteristics and meat quality in Wenchang broiler chickens[J]. Acta Ecologae Animalis Domastici, 2017, 38(10):33-37. (in Chinese)

[33]
盛子阳, 王定发, 吕仁龙, 等. 假蒟提取物对海南黑山羊体外瘤胃发酵参数和干物质消化率的影响[J]. 中国畜牧杂志, 2024, 60(5):233-238.

SHENG Z Y, WANG D F, LV R L, et al. The effect of false betel extract on in vitro rumen fermentation parameters and dry matter digestibility of Hainan black mountain sheep[J]. Chinese Journal of Animal Science, 2024, 60(5):233-238. (in Chinese)

[34]
盛子阳. 假蒟提取物改善海南黑山羊养分消化率机制初探[D]. 硕士学位论文. 北京: 中国农业大学, 2023.

SHENG Z Y. A preliminary mechanism study on the improving nutrient digestibility of Piper sarmentosum Roxb extract in Hainan black goat[D]. Master’s Thesis. Beijing: China Agricultural University, 2023. (in Chinese)

[35]
童雄, 闵力, 孙浩, 等. 雷州山羊、努比亚羊及其杂交F1代在热应激环境下生理和血液生化指标的对比研究[J]. 中国畜牧兽医, 2021, 48(10):3625-3634.

DOI

TONG X, MIN L, SUN H, et al. Comparative study on physiological and blood biochemical indexes of Leizhou goat, Nubian sheep and their hybrid F1 generation under heat stress[J]. China Animal Husbandry and Veterinary Medicine, 2021, 48(10):3625-3634. (in Chinese)

[36]
蔡冬宝. 矢车菊素-3-O-葡萄糖苷对热应激诱导的雄性生殖损伤的保护作用[D]. 硕士学位论文. 广州: 暨南大学, 2021.

CAI D B. The protective effects of cyanidin-3-O-glucoside on heat stress-induced male reproductive damage[D]. Master’s Thesis. Guangzhou: Jinan University, 2021. (in Chinese)

[37]
王世忠, 任怡敏, 姜俭, 等. 性成熟期前后睾丸及附睾碱性磷酸酶分布的观察[J]. 天津医科大学学报, 1999(1):26-28.

WANG S Z, REN Y M, JIANG J, et al. The observation on the distribution of the alp on the testes and the epididymises before and after sexual maturation phase[J]. Journal of Tianjin Medical University, 1999(1):26-28. (in Chinese)

[38]
HUANG Q, LIU Q, OUYANG D S. Sorbinil,an aldose reductase inhibitor,in fighting against diabetic complications[J]. Medicinal Chemistry, 2019, 15(1):3-7.

[39]
张适, 徐文山. 大鼠附睾中酶的组织化学观察[J]. 南京医学院学报, 1989(3):178-181,245.

ZHANG S, XU W S. Observations on the histochemistry of enzymes in the epididymis of rat[J]. Journal of Nanjing Medical University, 1989(3):178-181,245. (in Chinese)

[40]
桑润滋, 田树军, 李俊杰, 等. 热应激对荷斯坦种公牛精液品质的影响及机理[J]. 中国兽医学报, 2002, 22(4):407-410.

SANG R Z, TIAN S J, LI J J, et al. Influence of heat stress on semen quality of Holstein bull and approach to its mechanism[J]. Chinese Journal of Veterinary Science, 2002, 22(4):407-410. (in Chinese)

[41]
YARAHMADI P, MIANDARE H K, FAYAZ S, et al. Increased stocking density causes changes in expression of selected stress-and immune-related genes,humoral innate immune parameters and stress responses of rainbow trout (Oncorhynchus mykiss)[J]. Fish & Shellfish Immunology, 2016,48:43-53.

[42]
EINARSSON S, BRANDT Y, LUNDEHEIM N, et al. Stress and its influence on reproduction in pigs:a review[J]. Acta Veterinaria Scandinavica, 2008, 50(1):48.

[43]
LUE Y H, WANG C, LYDON J P, et al. Functional role of progestin and the progesterone receptor in the suppression of spermatogenesis in rodents[J]. Andrology, 2013, 1(2):308-317.

DOI PMID

[44]
O’SHAUGHNESSY P J, MONTEIRO A, ABEL M. Testicular development in mice lacking receptors for follicle stimulating hormone and androgen[J]. PLoS One, 2012, 7(4):e35136.

[45]
TODINI L, MALFATTI A, VALBONESI A, et al. Plasma total T3 and T4 concentrations in goats at different physiological stages,as affected by the energy intake[J]. Small Ruminant Research, 2007, 68(3):285-290.

[46]
SHAH W, KHAN R, SHAH B, et al. The molecular mechanism of sex hormones on sertoli cell development and proliferation[J]. Frontiers in Endocrinology, 2021,12:648141.

[47]
KOLUMAN N, DASKIRAN I. Effects of ventilation of the sheep house on heat stress,growth and thyroid hormones of lambs[J]. Tropical Animal Health and Production, 2011, 43(6):1123-1127.

[48]
BARAKAT B, ITMAN C, MENDIS S, et al. Activins and inhibins in mammalian testis development:new models,new insights[J]. Molecular and Cellular Endocrinology, 2012, 359(1/2):66-77.

[49]
姜志洋. 日粮添加姜黄素和槲皮素对夏季湖羊生产性能、血液指标和睾丸发育的影响[D]. 硕士学位论文. 南京: 南京农业大学, 2022.

JIANG Z Y. Effect of dietary curcumin and quercetin on production performance,blood parameters and testicular development of Hu sheep in summer[D]. Master’s Thesis. Nanjing: Nanjing Agricultural University, 2022. (in Chinese)

[50]
NAZIFI S, SAEB M, ROWGHANI E, et al. The influences of thermal stress on serum biochemical parameters of Iranian fat-tailed sheep and their correlation with triiodothyronine (T3),thyroxine (T4) and cortisol concentrations[J]. Comparative Clinical Pathology, 2003, 12(3):135-139.

[51]
马淑丽. 叶酸对中度热应激种公羊精液质量、血清抗氧化能力及内分泌激素的影响[D]. 硕士学位论文. 晋中: 山西农业大学, 2021.

MA S L. The effects of folic acid on semen quality,serum antioxidant capacity and endocrine hormones of ram under moderate heat stress[D]. Master’s Thesis. Jinzhong: Shanxi Agricultural University, 2021. (in Chinese)

[52]
DOORN J A, PETERSEN D R. Covalent adduction of nucleophilic amino acids by 4-hydroxynonenal and 4-oxononenal[J]. Chemico-Biological Interactions, 2003,143-144:93-100.

[53]
GANDHI S, ABRAMOV A Y. Mechanism of oxidative stress in neurodegeneration[J]. Oxidative Medicine and Cellular Longevity, 2012,2012:428010.

[54]
HAMILTON T R D S, SIQUEIRA A F P, DE CASTRO L S, et al. Effect of heat stress on sperm DNA:protamine assessment in ram spermatozoa and testicle[J]. Oxidative Medicine and Cellular Longevity, 2018,2018:5413056.

[55]
施力光, 周雄, 荀文娟, 等. 补饲硒和维生素E对高温季节山羊精液品质、抗氧化酶活性及热休克蛋白表达的影响[J]. 中国畜牧兽医, 2016, 43(1):101-107.

DOI

SHI L G, ZHOU X, XUN W J, et al. Effect of Se and VE supplement on semen quality, antioxidant enzyme activities and heat shock protein expression of goat in high temperature season[J]. China Animal Husbandry & Veterinary Medicine, 2016, 43(1):101-107. (in Chinese)

[56]
彭孝坤, 赵天, 黄晓瑜, 等. 急性热应激对山羊血液生化指标及血淋巴细胞热休克蛋白70家族基因表达的影响[J]. 畜牧兽医学报, 2019, 50(6):1219-1229.

PENG X K, ZHAO T, HUANG X Y, et al. Effects of acute heat stress on blood biochemistry indices and expression of HSP70 family genes in blood lymphocytes in goats[J]. Acta Veterinaria et Zootechnica Sinica, 2019, 50(6):1219-1229. (in Chinese)

DOI

[57]
RHOADS R P, BAUMGARD L H, SUAGEE J K, et al. Nutritional interventions to alleviate the negative consequences of heat stress[J]. Advances in Nutrition, 2013, 4(3):267-276.

DOI PMID

[58]
ZHAO J X, JIN Y Q, DU M, et al. The effect of dietary grape pomace supplementation on epididymal sperm quality and testicular antioxidant ability in ram lambs[J]. Theriogenology, 2017,97:50-56.

[59]
HUNYADI A. The mechanism(s) of action of antioxidants:from scavenging reactive oxygen/nitrogen species to redox signaling and the generation of bioactive secondary metabolites[J]. Medicinal Research Reviews, 2019, 39(6):2505-2533.

[60]
CHEN D, XIAO Z P, GUO H, et al. Identification of a bromodomain-like region in 15-lipoxygenase-1 explains its nuclear localization[J]. Angewandte Chemie (International ed. in English), 2021, 60(40):21875-21883.

[61]
MEHTA N U, GRIJALVA V, HAMA S, et al. Apolipoprotein E-/- mice lacking hemopexin develop increased atherosclerosis via mechanisms that include oxidative stress and altered macrophage function[J]. Arteriosclerosis Thrombosis and Vascular Biology, 2016, 36(6):1152-1163.

[62]
ZHAO H, ZHU Y Y, ZHAO Y F, et al. Alleviating effects of selenium on fluoride-induced testosterone synthesis disorder and reproduction toxicity in rats[J]. Ecotoxicology and Environmental Safety, 2022,247:114249.

[63]
SHAMSI M B, VENKATESH S, TANWAR M, et al. DNA integrity and semen quality in men with low seminal antioxidant levels[J]. Mutation Research, 2009, 665(1/2):29-36.

[64]
ZHOU L L, WANG D F, HU H C, et al. Effects of piper sarmentosum extract supplementation on growth performances and rumen fermentation and microflora characteristics in goats[J]. Journal of Animal Physiology and Animal Nutrition, 2020, 104(2):431-438.

DOI PMID

[65]
LEE S, MARGOLIN K. Cytokines in cancer immunotherapy[J]. Cancers, 2011, 3(4):3856-3893.

DOI PMID

[66]
李花. 番茄红素对小鼠睾丸热应激损伤保护机制研究[D]. 硕士学位论文. 内蒙古: 内蒙古医科大学, 2023.

LI H. Heat stress damage in mice by lycopene research on protection mechanism[D]. Master’s Thesis. Hohhot: Inner Mongolia Medical University, 2023. (in Chinese)

[67]
臧青民, 章烨雯, 李海东, 等. 假蒟及其提取物的生物活性及在畜禽养殖中的应用[J]. 饲料研究, 2021, 44(12):138-141.

ZANG Q M, ZHANG Y W, LI H D, et al. Bioactivity and application in livestock and poultry breeding of Piper sarmentosum Roxb and its extract[J]. Feed Research, 2021, 44(12):138-141. (in Chinese)

[68]
WANG D F, ZHOU L L, ZHOU H L, et al. Effects of Piper sarmentosum extract on the growth performance,antioxidant capability and immune response in weaned piglets[J]. Journal of Animal Physiology and Animal Nutrition, 2017, 101(1):105-112.

[69]
BANERJEE D, UPADHYAY R C, CHAUDHARY U B, et al. Seasonal variation in expression pattern of genes under HSP70:seasonal variation in expression pattern of genes under HSP70 family in heat-and cold-adapted goats (Capra hircus)[J]. Cell Stress and Chaperones, 2014, 19(3):401-408.

[70]
FEDER M E, HOFMANN G E. Heat-shock proteins,molecular chaperones,and the stress response:evolutionary and ecological physiology[J]. Annual Review of Physiology, 1999,61:243-282.

[71]
GARRIDO C, GURBUXANI S, RAVAGNAN L, et al. Heat shock proteins:endogenous modulators of apoptotic cell death[J]. Biochemical and Biophysical Research Communications, 2001, 286(3):433-442.

[72]
NEUER A, SPANDORFER S D, GIRALDO P, et al. The role of heat shock proteins in reproduction[J]. Human Reproduction Update, 2000, 6(2):149-159.

DOI PMID

Outlines

/