RESEARCH PAPER

Study on Roles of Mannan Oligosaccharides in Regulating Rumen Fermentation and Microbiota Structure in Vitro

  • CHANG Shuaifei ,
  • GUO Yunfang ,
  • CHENG Yuchen ,
  • REN Wenyi ,
  • LI Haibo ,
  • HE Jintong ,
  • KANG Yan ,
  • LIU Xiaonv ,
  • KONG Xiaoli ,
  • ZHANG Lili ,
  • XU Xiaofeng , *
Expand
  • College of Animal Science and Technology, Ningxia University, Yinchuan 750021, China
*professor, E-mail:

Received date: 2024-04-16

  Online published: 2024-10-14

Abstract

The aim of this experiment was to investigate the roles of mannan oligosaccharides in regulating rumen fermentation and microbiota structure in vitro. The trial was conducted in a completely randomized design and divided into four groups, with 0, 0.5%, 1.5% and 3.0% mannan oligosaccharides added into the fermentation broth in the control group (CON group), the low-dose group (LMO group), the medium-dose group (MMO group) and the high-dose group (HMO group), respectively, and 6 replicates were set in each group. The experiment was carried out using alfalfa hay as fermentation substrate, and in vitro rumen fermentation test was carried out to study the regulatory effects of mannan oligosaccharides on gas production parameters, fermentation parameters and microbiota structure. The results showed as follows: 1) compared with CON group, the 24 h cumulative gas production, theoretical maximum gas production and total volatile fatty acid concentration in MMO group were significantly increased (P<0.05); the 24 h cumulative gas production, gas generation rate and total volatile fatty acid concentration in HMO group were significantly increased (P<0.05), and the ammoniacal nitrogen (NH3-N) concentration was significantly decreased (P<0.05). There were no significant differences in the molar ratios of acetic acid and propionic acid as well as the acetic acid to propionic acid ratio among all groups (P>0.05). 2) Compared with CON group, the relative abundances of Firmicutes and Ruminococcus in HMO group were significantly increased (P<0.05), and the relative abundances of Prevotella_1 (P=0.065) and Christensenellaceae_R-7_group (P=0.075) tended to be increased. 3) The results of correlation analysis between rumen fermentation parameters and microbiota in vitro showed that the Firmicutes relative abundance was significantly positively correlated with the concentrations of acetic acid, propionic acid and total volatile fatty acid (P<0.05); the Ruminococcus relative abundance was significantly positively correlated with 24 h cumulative gas production, gas generation rate and concentrations of acetic acid, propionic acid and total volatile fatty acid (P<0.05), while significantly negatively correlated with NH3-N concentration (P<0.05). In conclusion, mannan oligosaccharides have positive effects on rumen fermentation in vitro, which can improve the Ruminococcus relative abundance and nitrogen utilization capacity, and increase the total volatile fatty acid production by regulating the structure of rumen microbiota, but does not change the fermentation pattern.

Cite this article

CHANG Shuaifei , GUO Yunfang , CHENG Yuchen , REN Wenyi , LI Haibo , HE Jintong , KANG Yan , LIU Xiaonv , KONG Xiaoli , ZHANG Lili , XU Xiaofeng . Study on Roles of Mannan Oligosaccharides in Regulating Rumen Fermentation and Microbiota Structure in Vitro[J]. Chinese Journal of Animal Nutrition, 2024 , 36(10) : 6588 -6598 . DOI: 10.12418/CJAN2024.560

甘露寡糖是近年来研究较多的一种功能性寡糖,其因较强的肠道菌群调节能力,被广泛应用于水产、单胃和反刍动物等多重领域[1-3]。Zhang等[4]研究表明,甘露寡糖能促进结肠炎小鼠的肠道微生态恢复。Bai等[5]研究表明,甘露寡糖能够正向调节高蛋白质饲粮下大菱鲆肠道菌群,并改善其生长性能。Yu等[6]研究表明,甘露寡糖可以改善断奶仔猪肠道微生物群落和肠道屏障功能。而在反刍动物方面,诸多饲养试验证实,甘露寡糖在优化瘤胃发酵进而提升动物生产性能方面有明显的作用,尤其是可以提升反刍动物对纤维物质的利用。Westland等[7]研究表明,在产前饲粮中添加甘露寡糖可以显著提升奶牛的初乳产量。Zhang等[8]研究表明,甘露寡糖能够促进牛粪菌群对稻草纤维素的利用。本课题组前期研究表明,甘露寡糖可以促进高精料诱导下的低乳脂奶牛的瘤胃菌群恢复,尤其是影响厚壁菌门(Firmicutes)、纤维杆菌门(Fibrobacteres)和瘤胃球菌属(Ruminococcus)等纤维降解菌群相对丰度的变化[9]。不过,目前针对甘露寡糖的报道多集中在体内,尚不清楚甘露寡糖的菌群调节作用是单独发生,还是与饲粮其他成分协同作用。苜蓿干草的营养价值高、适口性好,在瘤胃中有较高的降解率,是反刍动物饲粮中使用最广泛的粗饲料之一。本试验为简化干扰因素,仅使用苜蓿干草作为发酵底物,通过模拟瘤胃发酵,并监测其发酵参数以及菌群结构的变化,以此来研究甘露寡糖对瘤胃菌群的调控作用,以期为阐明甘露寡糖的调控机制提供理论依据。

1 材料与方法

1.1 试验设计

试验采用完全随机设计,共设置4个组,对照组(CON组)在发酵液中不添加甘露寡糖,试验组分别在发酵液中添加0.5%(低剂量组,LMO组)、1.0%(中剂量组,MMO组)和3.0%(高剂量组,HMO组)甘露寡糖,每组设置6个重复。通过研究产气参数和发酵参数变化,根据综合分析的比较结果,确定1个试验组进行24 h瘤胃菌群分析。

1.2 体外瘤胃发酵

1.2.1 发酵培养液的制备

将400 mL蒸馏水、0.1 mL A液、200 mL B液、200 mL C液、1 mL刃天青溶液和40 mL还原剂溶液混合均匀后即可制得缓冲液,缓冲液各组分的配制方案见表1。将配制好的缓冲液持续充入二氧化碳(CO2),待颜色变浅或无色后置于39 ℃水浴锅中备用。
表1 缓冲液各组分的配制方案

Table 1 Preparation scheme of each component in buffer solution

项目 Items 组成 Composition
A液 Liquid A CaCl2·2H2O 13.2 g、MnCl2·4H2O 10.0 g、CoCl2·6H2O 1.0 g、
FeCl3·6H2O 8.0 g,加蒸馏水定容至100 mL
B液 Liquid B NH4CO3 4.0 g、NaHCO3 35 g,加蒸馏水定容至1 000 mL
C液 Liquid C NaHPO4 5.7 g、KH2PO4 6.2 g、MgSO4·7H2O 0.6 g,加蒸馏水定容至1 000 mL
刃天青溶液 Resazurin solution 0.1 g刃天青,加蒸馏水定容至100 mL
还原剂溶液 Reductant solution 1 mol/L NaOH 4.0 mL,Na2S·9H2O 0.625 g,加蒸馏水至95 mL
按照试验设计在各组缓冲液中添加相应剂量的甘露寡糖(纯度≥95%)。选用3头装有瘤胃瘘管的健康中国荷斯坦奶牛作为瘤胃液供体,奶牛采用全混合日粮饲喂,饲粮精粗比为30∶70(风干基础),其组成及营养水平见表2。于晨饲后2 h在奶牛瘤胃的不同位置采集瘤胃液,混匀后装入充有CO2的保温瓶,迅速带回实验室。新鲜瘤胃液经4层纱布过滤后与缓冲液按2∶1的比例混合即可得发酵培养液。
表2 饲粮组成及营养水平(干物质基础)

Table 2 Composition and nutrient levels of the diet (DM basis)%

项目 Items 含量 Content
原料 Ingredients
玉米青贮 Corn silage 45.06
苜蓿青贮 Alfalfa silage 4.12
啤酒糟 Brewer’s grains 1.53
蒸汽压片玉米 Steam-flaked corn 22.50
苜蓿干草 Alfalfa hay 10.32
浓缩料 Concentrated feed1) 14.30
甜菜颗粒 Beet granules 2.00
碳酸氢钠 NaHCO3 0.17
合计 Total 100.00
营养水平 Nutrient levels2)
净能 NE/(MJ/kg) 5.94
粗蛋白质 CP 11.69
粗脂肪 EE 2.54
中性洗涤纤维 NDF 47.32
酸性洗涤纤维 ADF 30.74
钙 Ca 0.67
磷 P 0.28

1)浓缩料的营养水平如下 Nutrient levels of the concentrated feed were as follows:干物质 DM 86%,粗蛋白质 CP 29.5%,粗灰分 Ash 18%,粗纤维 CF 12%,钙 Ca 1.3%,总磷 TP 0.6%,氯化钠 NaCl 1.3%,赖氨酸 Lys 0.8%。每千克浓缩料含有 One kilogram of the concentrated feed contained the following:维生素A乙酸酯 vitamin A acetate 12 000 IU,VD3 3 300 IU,DL-α-生育酚乙酸酯 DL-α-tocopheryl acetate 4 200 mg,烟酰胺 nicotinamide 6 700 mg,Mn 6 200 mg,Fe 1 800 mg,Zn 8 900 mg,Cu 1 700 mg,Se 41.7 mg,I 120 mg,Co 90 mg/kg。

2)净能参照NRC(2001)计算所得,其余为实测值。NE was calculated by reference to NRC (2001), while the others were measured values.

1.2.2 瘤胃发酵试验

发酵管为100 mL玻璃注射器,最小刻度为1 mL。注射器前安装有带夹子的乳胶管来确保密封性,并在活塞表面涂抹凡士林来减少阻力和防止漏气。将苜蓿干草粉碎后,准确称取200 mg风干状态下的苜蓿草粉置于发酵管底部作为发酵底物。苜蓿干草的营养成分见表3。向各发酵管内加入30 mL发酵培养液后,倒置于充分预热的(39 ℃)水浴摇床内。设置空白组(无发酵底物,只添加发酵培养液)用于校正产气量。记录发酵管活塞的初始刻度值(mL),启动水浴摇床开始培养,进行24 h体外瘤胃发酵。
表3 苜蓿干草的营养成分(风干基础)

Table 3 Nutrients of alfalfa hay (air-dry basis)%

项目
Item
粗蛋
白质
CP
粗脂肪
EE
中性洗
涤纤维
NDF
酸性洗
涤纤维
ADF
淀粉
Starch
粗灰分
Ash

Ca

P
含量 Content 21.5 2.56 39.83 33.36 2.75 12.55 2.69 0.27

1.3 测定指标及方法

1.3.1 营养成分的测定

粗蛋白质(CP)含量采用全自动凯氏定氮仪(GB/T 6432—2018)进行测定,粗脂肪(EE)含量采用索氏提取法(GB/T 6433—2006)进行测定,粗灰分(Ash)、钙(Ca)和磷(P)含量分别参照国标GB/T 6438—2007、GB/T 6436—2018和GB/T 6437—2018方法进行测定。中性洗涤纤维(NDF)和酸性洗涤纤维(ADF)含量参照Van Soest等[10]的方法进行测定。淀粉含量参照国标GB/T 20194—2018方法进行测定。

1.3.2 产气参数的测定

分别记录发酵3、6、9、12和24 h时各发酵管的刻度值(mL)。某时间点的实际产气量等于该时间点活塞位置读数与该培养管初始读数之差。
产气参数根据陈延斌等[11]所述的动态发酵模型来计算,计算公式为:

GPt=B(1-e-ct)。

式中:GPtt时间点的累积产气量(mL);t为发酵时间(h);B为该时间点的理论最大产气值(mL);c为产气速率(%/h)。

1.3.3 瘤胃发酵参数的测定

发酵结束后,立即用冰水冷却发酵液,使用便携式pH计测量pH,随后将剩余发酵液全部置于-80 ℃冰箱中保存。采用比色法[12]测定发酵液氨态氮(NH3-N)浓度,利用日本岛津GC-2030气相色谱仪测定发酵液挥发性脂肪酸浓度[13]

1.3.4 微生物群落分析

将-80 ℃保存的CON组和HMO组发酵液样品送往广州基迪奥生物科技有限公司进行测序。先对样品进行DNA提取,然后以引物338F(5'-ACTCCTACGGGAGGCAGCA-3')和806R(5'-GGACTACHVGGGTWTCTAAT-3')对样品DNA进行PCR扩增。将PCR产物用1%琼脂糖凝胶电泳检测,再用Agencourt AMPure XP核酸纯化试剂盒进行分离纯化。利用Illumina HiSeq PE 2500平台对端测序,进行16S rDNA序列测定。筛选出97%以上相似度的序列,用于微生物多样性和组成分析。测序所得序列使用USEARCH 10.0软件将相似度超过97%的序列分配至一个操作分类单元(OTU)。OTU的分类注释利用QIIME 2软件中的Naïve Bayes分类器进行,分类基于SILVA数据库(138.1版本),其置信阈值为70%。微生物α多样性的分析使用QIIME 2软件进行。微生物的相对丰度和多样性差异使用t检验来比较分析。

1.4 数据统计与分析

采用SAS 9.4软件对除微生物群落的试验数据进行单因素方差分析(one-way ANOVA),并采用Duncan氏法进行多重比较,结果数据以平均值和均值标准误(SEM)表示,P<0.05表示差异显著,0.05≤P<0.10表示差异有显著趋势。

2 结果与分析

2.1 甘露寡糖对体外瘤胃发酵的影响

2.1.1 甘露寡糖对体外瘤胃发酵产气参数的影响

表4可知,与CON组相比,MMO组和HMO组24 h累积产气量均显著提高(P<0.05),分别提高了6.76%和6.15%;MMO组理论最大产气量显著提高(P<0.05),提高了5.25%;HMO组产气速率显著提高(P<0.05),提高了14.19%。
表4 甘露寡糖对体外瘤胃发酵产气参数的影响

Table 4 Effects of mannan oligosaccharides on gas production parameters of rumen fermentation in vitro

项目
Items
组别 Groups 均值标准误
SEM
P
P-value
CON LMO MMO HMO
24 h累积产气量
24 h cumulative gas production/mL
54.33b 53.67b 58.00a 57.67a 0.73 <0.001
理论最大产气量
Theoretical maximum gas production/mL
57.75b 56.68b 60.78a 59.41ab 0.69 <0.001
产气速率
Gas generation rate/(%/h)
0.14b 0.15ab 0.15ab 0.16a 0.01 0.039

同行数据肩标相同小写字母或无字母表示差异不显著(P>0.05),不同小写字母表示差异显著(P<0.05)。下表同。

In the same row, values with the same small letter or no letter superscript mean no significant difference (P>0.05), while with different small letter superscripts mean significant difference (P<0.05). The same as below.

2.1.2 甘露寡糖对体外瘤胃发酵参数的影响

表5可知,与CON组相比,MMO组和HMO组发酵液总挥发性脂肪酸浓度均显著提高(P<0.05),分别提高了6.90%和19.31%;HMO组发酵液NH3-N浓度显著降低(P<0.05),降低了4.44%。各组间发酵液乙酸、丙酸和丁酸摩尔比以及乙酸/丙酸值均无显著差异(P>0.05)。
表5 甘露寡糖对体外瘤胃发酵参数的影响

Table 5 Effects of mannan oligosaccharides on rumen fermentation parameters of in vitro

项目
Items
组别 Groups 均值标准误
SEM
P
P-value
CON LMO MMO HMO
pH 6.92 6.90 6.94 6.96 0.02 0.621
氨态氮 NH3-N/(mg/dL) 14.85a 14.94a 14.51ab 14.19b 0.11 0.043
总挥发性脂肪酸 TVFA/(mmol/L) 84.94b 90.64b 90.80a 101.34a 2.07 0.009
乙酸摩尔比 Acetic acid molar ratio/% 66.91 65.42 65.55 64.56 0.53 0.154
丙酸摩尔比 Propionate acid molar ratio/% 22.99 22.84 23.33 24.66 1.24 0.287
丁酸摩尔比 Butyric acid molar ratio/% 7.10 8.74 8.12 7.78 0.26 0.163
乙酸/丙酸 Acetic acid/propionic acid 2.79 2.84 2.93 3.05 0.30 0.235

2.2 甘露寡糖对体外瘤胃发酵液菌群的影响

2.2.1 甘露寡糖对体外瘤胃发酵液菌群α多样性的影响

在通过QIIME 2质控后,CON组和HMO组的12个样品总共生成1 502 691个raw tags以及1 331 934个effective tags。参考细菌数据库,所有序列以97%的相似水平聚类为23个门、300个属的OTU信息。根据每个样品的OTU总数及各个OTU的相对丰度进行样品多样性指数计算,由表6可知,CON组和HMO组的覆盖率都在99%以上,表明此次测序有足够的测序深度,测序数据能够反映样本的真实水平。与CON组相比,HMO组的Shannon、Simpson、Sobs、Chao1、Pielou、Ace和PD指数均无显著差异(P>0.05)。
表6 甘露寡糖对体外瘤胃发酵液菌群α多样性的影响

Table 6 Effects of mannan oligosaccharides on microbiota α diversity in rumen fermentation broth in vitro

项目
Items
组别 Groups 均值标准误
SEM
P
P-value
CON HMO
Shannon指数Shannon index 6.18 6.43 0.13 0.368
Simpson指数 Simpson index 0.94 0.94 0.01 0.866
Sobs指数 Sobs index 1 675.33 1 748.83 23.21 0.117
Chao1指数 Chao1 index 1 862.77 1 912.81 21.19 0.256
Pielou指数 Pielou index 0.58 0.60 0.01 0.422
Ace指数 Ace index 1 973.48 2 032.55 24.45 0.244
覆盖率 Coverage/% 99.36 99.58 <0.01 0.156
PD指数 PD index 180.74 192.59 3.81 0.124

2.2.2 甘露寡糖对体外瘤胃发酵液菌群组成的影响

表7可知,与CON组相比,HMO组发酵液厚壁菌门相对丰度显著提高(P<0.05),提高了19.36%,其他菌门相对丰度均无显著差异(P>0.05)。
表7 甘露寡糖对体外瘤胃发酵液菌群在门水平上组成的影响

Table 7 Effects of mannan oligosaccharides on microbiota composition at phylum level in rumen fermentation broth in vitro%

项目
Items
组别 Groups 均值标准误
SEM
P
P-value
CON HMO
厚壁菌门 Firmicutes 40.09b 47.85a 1.82 0.024
变形菌门 Proteobacteria 23.35 19.50 2.66 0.490
拟杆菌门 Bacteroidetes 19.83 22.16 0.86 0.189
Epsilonbacteraeota 12.05 8.58 2.33 0.483
广古菌门 Euryarchaeota 1.60 0.81 0.30 0.200
髌骨菌门 Patescibacteria 1.12 1.18 0.05 0.593
表8可知,与CON组相比,HMO组发酵液瘤胃球菌属(Ruminococcus)相对丰度显著提高(P<0.05),提高了24.83%;普雷沃氏菌属1(Prevotella_1)(P=0.065)和克里滕森菌科R-7群(Christensenellaceae_R-7_group)(P=0.075)相对丰度有提高的趋势,分别提高了16.58%和47.19%;其他菌属相对丰度均无显著差异(P>0.05)。
表8 甘露寡糖对体外瘤胃发酵液菌群在属水平上组成的影响

Table 8 Effects of mannan oligosaccharides on microbiota composition at genus level in rumen fermentation broth in vitro%

项目
Items
组别 Groups 均值标准误
SEM
P
P-value
CON HMO
土壤芽孢杆菌属 Solibacillus 10.38 12.24 1.82 0.634
普雷沃氏菌属1 Prevotella_1 10.19 11.88 0.47 0.065
弯曲杆菌属 Campylobacter 12.05 7.41 2.15 0.302
从毛单胞菌属 Comamonas 10.55 6.56 2.45 0.443
埃希氏-志贺氏菌属 Escherichia-Shigella 6.79 9.12 1.25 0.375
赖氨酸芽孢杆菌属 Lysinibacillus 7.38 5.40 0.97 0.332
解琥珀酸菌属 Succiniclasticum 4.95 5.59 0.41 0.467
理研菌科RC9肠道群
Rikenellaceae_RC9_gut_group
3.76 4.15 0.23 0.426
瘤胃球菌属 Ruminococcus 2.98b 3.72a 0.18 0.030
链球菌属 Streptococcus 1.56 4.36 1.04 0.191
克里斯藤森菌科R-7群
Christensenellaceae_R-7_group
1.78 2.62 0.24 0.075
库特氏菌属 Kurthia 1.69 1.31 0.48 0.706
月形单胞菌属1 Selenomonas_1 1.45 1.44 0.06 0.906
甲烷短杆菌属 Methanobrevibacter 1.59 0.80 0.30 0.199
不动杆菌属 Acinetobacter 1.38 0.99 0.47 0.698

2.3 体外瘤胃发酵参数与发酵液菌群相关性分析

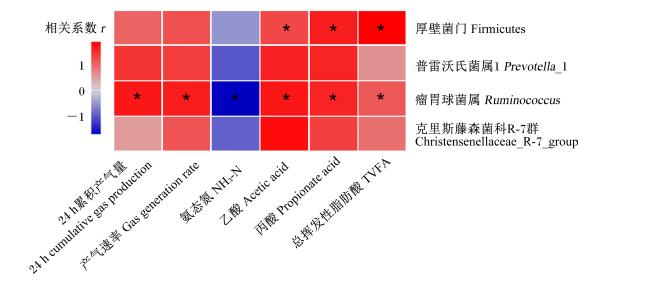
将体外瘤胃发酵参数与发酵液菌群相对丰度进行Spearman相关性分析,结果用热图展示(图1),结果表明,厚壁菌门相对丰度与发酵液乙酸、丙酸和总挥发性脂肪酸浓度均呈显著正相关(P<0.05);瘤胃球菌属相对丰度与24 h累积产气量、产气速率以及乙酸、丙酸和总挥发性脂肪酸浓度均呈显著正相关(P<0.05),与发酵液NH3-N浓度呈显著负相关(P<0.05)。
图1 体外瘤胃发酵参数与发酵液菌群相关性分析

*表示显著相关(P<0.05)。

Fig.1 Correlation analysis between rumen fermentation parameters and microbiota in fermentation broth in vitro

* indicated significant correlation (P<0.05).

3 讨论

3.1 甘露寡糖对体外瘤胃发酵参数的影响

反刍动物的瘤胃是一个高效的“生物反应器”。大量的瘤胃微生物将饲粮中的碳水化合物转化为挥发性脂肪酸来为宿主供能,同时还会产生各种气体。发酵液中挥发性脂肪酸浓度和产气量可以综合反映瘤胃微生物对饲粮的降解程度[14]。本试验中,添加1.5%和3.0%甘露寡糖均显著提高了体外瘤胃发酵24 h累积产气量和总挥发性脂肪酸浓度。甘露寡糖对瘤胃的挥发性脂肪酸产量有积极影响,郭婷婷[9]研究表明,在奶牛饲粮中添加200 g/(d·头)的甘露寡糖后,瘤胃总挥发性脂肪酸浓度显著提高,这与本研究结果一致。马秀花等[15]研究表明,在荞麦秸秆饲粮中添加1%和2%的甘露寡糖能够显著提高瘤胃液乙酸浓度。陈志龙等[16]研究表明,添加2%甘露寡糖提高了不同饲粮体外发酵的乙酸浓度,但差异不显著。肖宇[17]研究表明,在奶山羊饲粮中添加1%的甘露寡糖提高了瘤胃乙酸和总挥发性脂肪酸浓度,但差异不显著。酵母壁中含有约30%的甘露寡糖,在断奶仔猪饲粮中添加0.45%的酵母壁多糖显著提高了仔猪结肠乙酸和丙酸浓度[18]。体外发酵过程中产气量的多少与微生物活力直接相关。白天天等[19]报道了不同活力的屎肠球菌对体外瘤胃发酵的影响,在体外发酵过程中添加1×1010 CFU/mL的屎肠球菌可以使24 h产气量增加1.2倍。甘露寡糖对瘤胃微生物的活力有积极影响,研究表明,饲粮中添加甘露寡糖可以使锦江黄牛瘤胃液细菌种类和稳定性明显增加[20],饲料中添加甘露寡糖可以显著提高珍珠龙胆石斑鱼肠道菌群活力和多样性[21],饲粮中添加甘露寡糖可以显著改善低乳脂奶牛瘤胃菌群活力[9]。此外,祁茹等[22]研究表明,甘露寡糖可以显著增加瘤胃液中细菌总数以及纤维素分解菌、原虫和真菌数量。
NH3-N是反映瘤胃微生物对含氮物质的降解以及摄取利用的重要指标[16]。大多数的瘤胃细菌,如嗜淀粉瘤胃杆菌(Ruminobacter amylophilus)、溶纤维丁酸弧菌(Butyrivibrio fibrisolvens)和栖瘤胃普雷沃氏菌(Prevotella ruminicola),都具有蛋白酶活性[23]。在本试验中,添加甘露寡糖对体外瘤胃发酵NH3-N浓度产生了显著影响,且甘露寡糖添加量越高,NH3-N浓度越低,表明甘露寡糖提高了瘤胃微生物对氮的利用。然而,陈志龙等[16]研究表明,绵羊饲粮的体外发酵过程中添加甘露寡糖后NH3-N浓度显著升高。这2个试验结果不一致的现象可能与发酵底物的可发酵碳水化合物含量有关。本试验使用的苜蓿干草的可发酵碳水化合物含量较低,这使某些微生物增殖受阻,导致含氮物质的降解缓慢。同时,有研究表明,瘤胃普雷沃氏菌更倾向于利用NH3-N和肽作为氮源,而不是游离氨基酸[24]。本试验观测到试验组普雷沃氏菌属1相对丰度升高,NH3-N浓度的降低可能是由于甘露寡糖促进了普雷沃氏菌的增殖而引起。环境酸胁迫对微生物的生长繁殖有较大影响,当瘤胃内pH由6.5下降到5.8时,瘤胃菌群密度显著下降[25]。在本试验发酵培养液的配制中添加了较多的缓冲物质(NH4HCO3、NaHCO3和Na2HPO4),所以虽然总挥发性脂肪酸浓度显著提高,但发酵液pH并无显著变化。

3.2 甘露寡糖对体外瘤胃发酵液菌群的影响

在细菌门水平上,厚壁菌门是瘤胃内参与纤维物质降解的主要类群,目前对牛瘤胃中纤维素降解的研究主要集中在厚壁菌门中分离的少数菌株,即白色瘤胃球菌(Ruminococcus albus)和黄色瘤胃球菌(Ruminococcus flavefaciens)。很多研究报道了厚壁菌门与粗饲料降解的相关关系。赵烨嬋等[26]研究报道,呼伦贝尔羊采食干草后的瘤胃厚壁菌门相对丰度显著高于新生期。郑会超等[27]研究表明,当燕麦草在瘤胃中发酵2 h后,厚壁菌门和拟杆菌门即取代变形菌门成为附着在燕麦草中的优势菌门。在本试验中,添加3%的甘露寡糖使发酵液厚壁菌门相对丰度显著升高。在体内条件下也有相同的试验结果,在奶牛饲粮中添加200 g/(d·头)[9]和在滩羊的荞麦秸秆饲粮中添加2%的甘露寡糖[15]均显著提高了瘤胃液厚壁菌门的相对丰度。
在细菌属水平上,瘤胃球菌属是瘤胃内主要的纤维降解菌,瘤胃球菌属的很多菌株(如黄色瘤胃球菌)都可以降解十分牢固的纤维素种类,如棉花纤维[28]。反刍动物瘤胃中有大量瘤胃球菌属来源糖苷水解酶第48家族(GH48)基因序列,并且这些基因有丰富的多样性[29]。而GH48成员是外切葡聚糖酶的重要来源之一,可以通过和其他糖苷水解酶形成纤维小体或者自由酶体系2种方式来降解纤维素[30]。本试验中,添加3%甘露寡糖的发酵液瘤胃球菌属相对丰度显著提高,表明甘露寡糖对瘤胃球菌属的增殖有明显的促进作用。郭婷婷[9]和马秀花等[15]的研究也证实了这一观点,在奶牛和滩羊饲粮中添加甘露寡糖均可显著提高瘤胃球菌属的相对丰度。有研究表明,普雷沃氏菌属的碳水化合物降解能力与一种被称为多糖利用位点(PULs)的基因簇有关[31]。PULs主要作用于淀粉、半纤维素和果胶,有助于从半纤维素基质中释放纤维素[32]。在奶牛进食后2 h时,普雷沃氏菌属1是附着于燕麦草相对丰度最高的菌属,占总菌的19.23%,且相对丰度随着时间的延长不断升高,在进食后12 h时相对丰度达到22.60%;克里斯藤森菌科R-7群同样是最早附着于燕麦草的优势菌属,在奶牛进食后2 h时,其相对丰度达到5.91%[27]。克里斯藤森菌科R-7群具有降解植物多糖的潜力,其相对丰度在不同纤维底物的发酵液中发生显著变化[33]。奶牛饲粮中添加甘露寡糖后克里斯藤森菌科R-7群相对丰度显著提高[9],滩羊饲粮中添加甘露寡糖后普雷沃氏菌属相对丰度显著提高[15],本试验进一步证实了甘露寡糖对这2个菌属的积极影响。

3.3 体外瘤胃发酵参数与发酵液菌群相关性分析

在全基因组测序出现以前,微生物的功能特征主要通过形态学和生物化学等来确定。基因组测序可将细菌和古菌群落与重要瘤胃功能相关联,使用16S rRNA基因确定微生物分类后,通过与基因组关联,可将微生物种类与瘤胃功能联系起来。厚壁菌门是能够将植物多糖转变为挥发性脂肪酸的有益细菌,已经有一些研究揭示了厚壁菌门相对丰度与挥发性脂肪酸浓度之间的相关关系。刘依莎等[34]研究表明,在肉牛饲粮中添加20%的发酵玉米芯后,瘤胃厚壁菌门相对丰度显著降低,瘤胃总挥发性脂肪酸浓度也显著降低。在林波等[36]的研究中,泌乳水牛饲粮中添加烟酸后,瘤胃厚壁菌门相对丰度显著降低,瘤胃总挥发性脂肪酸浓度也随之显著降低。本试验证实了厚壁菌门相对丰度与挥发性脂肪酸浓度之间呈显著正相关关系。瘤胃球菌属是厚壁菌门的重要菌属,该菌属成员表现出卓越的植物多糖降解能力,不仅有降解纤维的白色瘤胃球菌和黄色瘤胃球菌,还有高效利用淀粉的嗜淀粉瘤胃球菌[36]。王亚玲等[37]研究表明,瘤胃内乙酸浓度与瘤胃球菌属相对丰度呈显著正相关关系。本试验证实了瘤胃球菌属相对丰度与乙酸浓度呈显著正相关,并且瘤胃球菌属相对丰度还与丙酸和总挥发性脂肪酸浓度、产气速率和24 h累积产气量均呈显著正相关,与NH3-N浓度呈显著负相关。

4 结论

在苜蓿干草的体外瘤胃发酵过程中添加3.0%甘露寡糖,可以调控发酵液菌群结构,提高瘤胃球菌属相对丰度,并提高产气速率和瘤胃氮利用能力,增加总挥发性脂肪酸产量,但对乙酸、丙酸、丁酸摩尔比以及乙酸/丙酸值无显著影响,不改变发酵模式。
[1]
KANGO N, JANA U K, CHOUKADE R, et al. Advances in prebiotic mannooligosaccharides[J]. Current Opinion in Food Science, 2022,47:100883.

[2]
LU Z Y, JIANG W D, WU P, et al. Cellular antioxidant mechanism of mannan-oligosaccharides involving in enhancing flesh quality in grass carp (Ctenopharyngodon idella)[J]. Journal of the Science of Food and Agriculture, 2023, 103(3):1172-1182.

[3]
JANA U K, SURYAWANSHI R K, PRAJAPATI B P, et al. Prebiotic mannooligosaccharides:synthesis,characterization and bioactive properties[J]. Food Chemistry, 2021,342:128328.

[4]
ZHANG T, CHENG T T, GENG S, et al. Synbiotic combination between Lactobacillus paracasei VL8 and mannan-oligosaccharide repairs the intestinal barrier in the dextran sulfate sodium-induced colitis model by regulating the intestinal stem cell niche[J]. Journal of Agricultural and Food Chemistry, 2024, 72(4):2214-2228.

[5]
BAI N, GU M, XU X J, et al. Protective effects of mannan oligosaccharides on turbot Scophthalmus maximus suffering from soy enteropathy[J]. Aquaculture, 2017,476:141-151.

[6]
YU E, CHEN D W, YU B, et al. Alteration of porcine intestinal microbiota in response to dietary manno-oligosaccharide supplementation[J]. Frontiers in Microbiology, 2021,12:811272.

[7]
WESTLAND A, MARTIN R, WHITE R, et al. Mannan oligosaccharide prepartum supplementation:effects on dairy cow colostrum quality and quantity[J]. Animal, 2017, 11(10):1779-1782.

[8]
ZHANG Y H, DUAN M L, ZHOU B B, et al. Mechanism that allows manno-oligosaccharide to promote cellulose degradation by the bacterial community and the composting of cow manure with straw[J]. Environmental Science and Pollution Research International, 2022, 29(20):30265-30276.

DOI PMID

[9]
郭婷婷. 甘露寡糖对高精料诱导的低乳脂奶牛瘤胃发酵及乳脂调控的研究[D]. 硕士学位论文. 银川: 宁夏大学, 2019.

GUO T T. Effects of mannan oligosaccharides on rumen fermentation and milk fat regulation of low milk fat dairy cows induced by high concentrate[D]. Master’s Thesis. Yinchuan: Ningxia University, 2019. (in Chinese)

[10]
VAN SOEST P J, ROBERTSON J B, LEWIS B A. Methods for dietary fiber,neutral detergent fiber,and nonstarch polysaccharides in relation to animal nutrition[J]. Journal of Dairy Science, 1991, 74(10):3583-3597.

[11]
陈延斌, 陈雅坤, 刘温, 等. 体外产气法评价不同质量分级评分等级的全株玉米青贮的饲用价值[J]. 动物营养学报, 2023, 35(5):3382-3389.

DOI

CHEN Y B, CHEN Y K, LIU W, et al. Evaluation of feeding value of whole-plant corn silage with different quality score grades by in vitro gas production method[J]. Chinese Journal of Animal Nutrition, 2023, 35(5):3382-3389. (in Chinese)

[12]
冯宗慈, 高民. 通过比色测定瘤胃液氨氮含量方法的改进[J]. 畜牧与饲料科学, 2010(6):37.

FENG Z C. Improvement of the method for determining the ammonia-nitrogen content of rumen liquor by colourimetry[J]. Animal Husbandry and Feed Science, 2010(6):37. (in Chinese)

[13]
李娅楠. 乳杆菌与地衣芽孢杆菌复合微贮对稻草营养价值影响及机理研究[D]. 硕士学位论文. 银川: 宁夏大学, 2022.

LI Y N. Effect and mechanism research of compound silage of lactobacillus and bacillus licheniformis on nutritional value of rice straw[D]. Master’s Thesis. Yinchuan: Ningxia University, 2022. (in Chinese)

[14]
IQBAL M W, ZHANG Q, YANG Y B, et al. Ruminal fermentation and microbial community differently influenced by four typical subtropical forages in vitro[J]. Animal Nutrition, 2018, 4(1):100-108.

[15]
马秀花, 桂瑞麒, 焦娜, 等. 荞麦秸秆饲粮条件下甘露寡糖对滩羊瘤胃菌群结构的影响[J]. 动物营养学报, 2021, 33(4):2365-2377.

DOI

MA X H, GUI R Q, JIAO N, et al. Effect of mannan oligosaccharides on rumen bacterial flora structure of Tan sheep under buckwheat straw diet condition[J]. Chinese Journal of Animal Nutrition, 2021, 33(4):2365-2377. (in Chinese)

[16]
陈志龙, 曾燕霞, 王林, 等. 不同精粗比饲粮中添加甘露寡糖对绵羊体外瘤胃发酵的影响[J]. 动物营养学报, 2016, 28(10):3292-3300.

DOI

CHEN Z L, ZENG Y X, WANG L, et al. Effects of mannanoligosaccharides supplementation in diets with different concentrate to roughage ratios on in vitro ruminal fermentation of sheep[J]. Chinese Journal of Animal Nutrition, 2016, 28(10):3292-3300. (in Chinese)

[17]
肖宇. 功能性寡糖对山羊瘤胃发酵参数及血清生化和免疫指标的影响[D]. 硕士学位论文. 青岛: 青岛农业大学, 2012.

XIAO Y. Effects of functional oligosaccharides on rumen fermentation,serum biochemical and immune indices of goats[D]. Master’s Thesis. Qingdao: Qingdao Agricultural University, 2012. (in Chinese)

[18]
贺琴. 酵母壁多糖对断奶仔猪生长性能、肠道微生物和机体免疫的影响[D]. 硕士学位论文. 南昌: 江西农业大学, 2017.

HE Q. Effect of yeast cell wall polysaccharides on growth performance,gut microbes and immune function of weaned piglets[D]. Master’s Thesis. Nanchang: Jiangxi Agricultural University, 2017. (in Chinese)

[19]
白天天, 崔浩然, 蒋辰宇, 等. 体外产气法比较不同活力屎肠球菌对绵羊瘤胃体外发酵的影响[J]. 动物营养学报, 2021, 33(11):6483-6491.

DOI

BAI T T, CUI H R, JIANG C Y, et al. Comparison of effects of enterococcus faecium with different activities on rumen in vitro fermentation in sheep using in vitro gas production method[J]. Chinese Journal of Animal Nutrition, 2021, 33(11):6483-6491. (in Chinese)

[20]
闵力. 功能性寡糖组合对锦江黄牛瘤胃微生物区系的影响[D]. 硕士学位论文. 南昌: 江西农业大学, 2012.

MIN L. Effects of functional oligosaccharides combination on rumen microflora of Jinjiang cattle[D]. Master’s Thesis. Nanchang: Jiangxi Agricultural University, 2012. (in Chinese)

[21]
王红明, 丁雪婧, 陈俭, 等. 饲料中添加甘露寡糖对珍珠龙胆石斑鱼生长性能、血清免疫指标、转录组及肠道菌群的影响[J]. 动物营养学报, 2021, 33(12):6982-6998.

DOI

WANG H M, DING X J, CHEN J, et al. Effects of dietary mannan-oligosaccharides on growth performance,serum immune indices,transcriptome and intestinal microflora of Epinephelus fuscoguttatus♀×Epinephelus lanceolatus ♂[J]. Chinese Journal of Animal Nutrition, 2021, 33(12):6982-6998. (in Chinese)

[22]
祁茹, 温建新, 程明, 等. 不同外源寡糖对崂山奶山羊瘤胃微生物区系的影响[J]. 动物营养学报, 2012, 24(2):349-357.

QI R, WEN J X, CHENG M, et al. Different exogenous oligosaccharides affect rumen microflora of Laoshan dairy goats[J]. Chinese Journal of Animal Nutrition, 2012, 24(2):349-357. (in Chinese)

[23]
WOZNY M A, BRYANT M P, HOLDEMAN L V, et al. Urease assay and urease-producing species of anaerobes in the bovine rumen and human feces[J]. Applied and Environment Microbiology, 1977, 33(5):1097-1104.

[24]
HAMMAD M I, CONRADS G, ABDELBARY M M H. Isolation,identification,and significance of salivary Veillonella spp.,Prevotella spp.,and Prevotella salivae in patients with inflammatory bowel disease[J]. Frontiers in Cellular and Infection Microbiology, 2023,13:1278582.

[25]
张丽, 李川, 邱清华, 等. 不同pH下瘤胃微生物菌群密度及理化特性的变化[J]. 动物营养学报, 2023, 35(1):450-459.

DOI

ZHANG L, LI C, QIU Q H, et al. Changes of rumen microbiota density and physicochemical properties at different pH[J]. Chinese Journal of Animal Nutrition, 2023, 35(1):450-459. (in Chinese)

DOI

[26]
赵烨嬋, 欧慧敏, 谭支良, 等. 呼伦贝尔羊不同生长阶段瘤胃微生物变化与羊肉膻味相关微生物分析[J]. 动物营养学报, 2024, 36(2):1050-1062.

DOI

ZHAO Y C, OU H M, TAN Z L, et al. Microbial changes in rumen of Hulun Buir sheep at different growth stages and analysis of odor-associated microbial communities[J]. Chinese Journal of Animal Nutrition, 2024, 36(2):1050-1062. (in Chinese)

[27]
郑会超, 郭晓辉, 蒋永清, 等. 燕麦草在奶牛瘤胃中的降解规律与黏附细菌区系变化[J]. 动物营养学报, 2023, 35(11):7201-7211.

DOI

ZHENG H C, GUO X H, JIANG Y Q, et al. Degradation regularity of oat grass in rumen of dairy cows and changes of attached bacterial flora[J]. Chinese Journal of Animal Nutrition, 2023, 35(11):7201-7211. (in Chinese)

DOI

[28]
STEWART C S, DUNCAN S H, FLINT H J. The properties of forms of Ruminococcus flavefaciens which differ in their ability to degrade cotton cellulose[J]. FEMS Microbiology Letters, 1990, 72(1/2):47-50.

[29]
李劲亭, 苏小运, 田彦, 等. 瘤胃细菌GH48家族糖苷水解酶基因多样性[J]. 微生物学报, 2014, 54(1):53-61.

LI J T, SU X Y, TIAN Y, et al. Gene diversity of the bacterial 48 family glycoside hydrolase (GH48) in rumen environment[J]. Acta Microbiologica Sinica, 2014, 54(1):53-61. (in Chinese)

[30]
OLSON D G, TRIPATHI S A, GIANNONE R J, et al. Deletion of the Cel48S cellulase from Clostridium thermocellum[J]. Proceedings of the National Academy of Sciences of the United States of America, 2010, 107(41):17727-17732.

[31]
MARTENS E C, CHIANG H C, GORDON J I. Mucosal glycan foraging enhances fitness and transmission of a saccharolytic human gut bacterial symbiont[J]. Cell Host & Microbe, 2008, 4(5):447-457.

[32]
STEWART R D, AUFFRET M D, WARR A, et al. Assembly of 913 microbial genomes from metagenomic sequencing of the cow rumen[J]. Nature Communications, 2018, 9(1):870.

DOI PMID

[33]
TAO S Y, BAI Y, ZHOU X J, et al. In vitro fermentation characteristics for different ratios of soluble to insoluble dietary fiber by fresh fecal microbiota from growing pigs[J]. ACS Omega, 2019, 4(12):15158-15167.

[34]
刘依莎, 张巧娥, 许迟, 等. 发酵玉米芯对肉牛生长性能、瘤胃发酵参数及菌群的影响[J]. 动物营养学报, 2024, 36(2):1039-1049.

DOI

LIU Y S, ZHANG Q E, XU C, et al. Effects of fermented corn cob on growth performance,rumen fermentation parameters and microflora of beef cattle[J]. Chinese Journal of Animal Nutrition, 2024, 36(2):1039-1049. (in Chinese)

[35]
林波, 梁辛, 韦升菊, 等. 烟酸对水牛瘤胃发酵指标及微生物区系的影响[J]. 动物营养学报, 2015, 27(8):2396-2404.

DOI

LIN B, LIANG X, WEI S J, et al. Effects of niacin on ruminal fermentation indexes and microflora of water buffaloes[J]. Chinese Journal of Animal Nutrition, 2015, 27(8):2396-2404. (in Chinese)

[36]
GAFFNEY J, EMBREE J, GILMORE S, et al. Ruminococcus bovis sp.nov.,a novel species of amylolytic Ruminococcus isolated from the rumen of a dairy cow[J]. International Journal of Systematic and Evolutionary Microbiology, 2021, 71(8):004924.

[37]
王亚玲, 孔鹏辉, 袁冬冬, 等. 饲粮添加乙酸钠对奶山羊泌乳性能和瘤胃微生物区系的影响[J]. 动物营养学报, 2023, 35(1):428-438.

DOI

WANG Y L, KONG P H, YUAN D D, et al. Effects of dietary sodium acetate on lactation performance and rumen microbiota of dairy goats[J]. Chinese Journal of Animal Nutrition, 2023, 35(1):428-438. (in Chinese)

DOI

Outlines

/