REVIEW

Research Progress on Protective Effects of Chitosan Oligosaccharides on Intestinal Mucosal Barrier Function

  • WANG Haoxuan ,
  • ZHANG Jia ,
  • LAN Ruixia , *
Expand
  • College of Coastal Agricultural Sciences, Guangdong Ocean University, Zhanjiang 524088, China
* lecturer, E-mail:

Received date: 2024-04-22

  Online published: 2024-11-09

Abstract

Chitosan oligosaccharides are the only alkaline amino oligosaccharides that exist in large quantity in nature. Chitosan oligosaccharides have antioxidant, anti-inflammatory, antibacterial and other biological functions, and can be used as safe and effective feed additives in animal diets. At present, the research on chitosan oligosaccharides mainly focuses on the growth performance, antioxidant and immune function in livestock and poultry. In recent years, studies have shown that chitosan oligosaccharides also have protective effects on intestinal damage, so they have been widely concerned. This article reviewed the biological functions of chitosan oligosaccharides and their protective effects on intestinal mucosal barrier function, aiming to provide theoretical references for the application of chitosan oligosaccharides in livestock and poultry production.

Cite this article

WANG Haoxuan , ZHANG Jia , LAN Ruixia . Research Progress on Protective Effects of Chitosan Oligosaccharides on Intestinal Mucosal Barrier Function[J]. Chinese Journal of Animal Nutrition, 2024 , 36(11) : 6917 -6928 . DOI: 10.12418/CJAN2024.590

现代养殖生产中,应激导致肠道上皮细胞受损、肠道消化吸收能力减弱以及饲料利用率下降,对动物生长和健康产生不良影响,造成巨大经济损失[1-2]。壳寡糖(chitosan oligosaccharides,COS)的原料甲壳素是除纤维素外最丰富的天然资源,是蟹、虾等甲壳类动物外壳的主要成分[3]。壳寡糖具有低分子质量、较高脱乙酰度、较高聚合度、较低黏性和完全水溶性,且具有广泛的生物活性,包括抗氧化、抗炎、抗肥胖、神经保护、抗癌和抗菌作用[4-6]。肠上皮细胞受损的根本原因是肠上皮间通透性增加,大分子物质、细菌能通过细胞旁路途径进入体内其他组织或体循环,从而诱导炎症反应,引发肠道疾病[7-8]。有些研究结果提出了许多缓解应激的策略,例如提供合适的环境、给予养分充足的饲粮,其中营养调控已被证实可有效缓解应激的负面作用[9]。近年研究表明,饲粮添加壳寡糖能够缓解环境应激对动物的肠道损伤,通过增强肠道抗氧化和抗炎能力,降低肠道通透性,维持肠道黏膜屏障功能[10-12]。本文简要介绍了壳寡糖的结构,并重点综述了壳寡糖生物学功能以及其在肠道黏膜屏障方面的保护作用,以期为壳寡糖在生产中的应用提供参考。

1 壳寡糖的结构和生物学功能

1.1 壳寡糖的结构
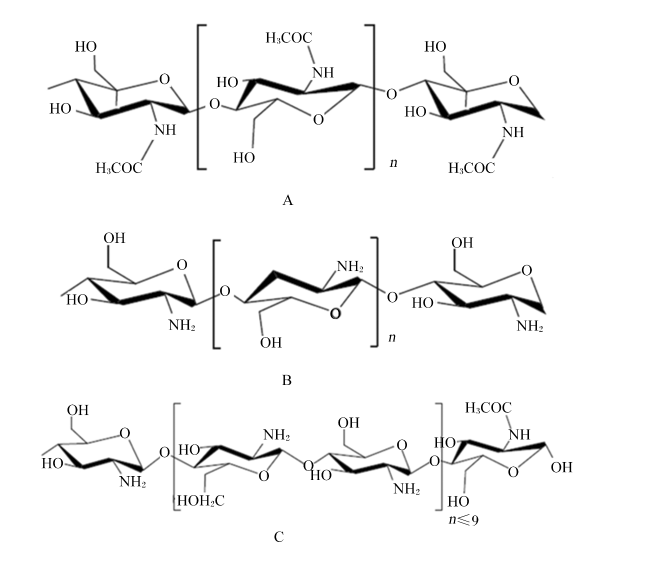
壳寡糖是一种功能性益生元,是聚合度小于20,平均分子质量低于3.9 ku,由2~10个氨基葡萄糖通过β-1,4-糖苷键连接的低聚寡糖,是自然界唯一大量存在的碱性氨基寡糖[13]。甲壳素(图1-A)经脱乙酰化转变为壳聚糖(图1-B),壳聚糖再通过降解转变为壳寡糖(图1-C)[14]
图1 甲壳素(A)、壳聚糖(B)和壳寡糖(C)分子结构

Fig.1 Molecular structures of chitin (A), chitosan (B) and chitosan oligosaccharides (C)[14]

1.2 壳寡糖的生物学功能

1.2.1 抗氧化功能

外界环境变化会诱导动物机体产生大量自由基,最终导致氧化应激[15],机体受到损伤[16]。壳寡糖的结构松散,分子内氢键相对较弱,氨基能与不稳定自由基反应形成稳定自由基,乙酰氨基和羟基官能团能抑制自由基对脂质、蛋白质和DNA等大分子的攻击作用,从而产生抗氧化效果[17]。何雪萍[18]报道,壳寡糖可提高黄羽肉鸡血清过氧化氢酶(catalase,CAT)以及肝脏超氧化物歧化酶(superoxide dismutase,SOD)和谷胱甘肽过氧化物酶(glutathione peroxidase,GSH-Px)活性,降低肝脏丙二醛(malondialdehyde,MDA)含量,缓解黄羽肉鸡的氧化应激。Xu等[19]报道,壳寡糖能提高蛋鸡血清总抗氧化能力(total antioxidant capacity,T-AOC),降低血清MDA含量,清除体内羟自由基(OH-·)、超氧阴离子自由基( O 2 -·)和过氧化氢(H2O2)等自由基,提高机体抵抗氧化能力。Lan等[20]报道,壳寡糖能降低卷毛鸡胸肌和腿肌MDA含量,提高SOD、CAT和GSH-Px活性,并提高1,1-二苯基-2-三硝基苯肼(1,1-diphenyl-2-picryl-hydrazyl radical,DPPH)、 O 2 -·、OH-·、2,2'-联氮-二(3-乙基-苯并噻唑-6-磺酸)二铵盐[ABTS]清除活性,提高胸肌和腿肌核因子红系2相关因子2(nuclear factor erythroid 2-related factor 2,Nrf2)、SOD、NAD(P)H:醌氧化还原酶1[NAD(P)H:quinone oxidoreductase 1,NQO1]、血红素加氧酶-1(heme oxygenase-1,HO-1)和GSH-Px基因的相对表达量。这些研究结果表明,壳寡糖能清除体内多余的自由基,增强抗氧化酶活性,提高抗氧化酶相关基因的表达,进而提高抗氧化作用。

1.2.2 抗炎功能

硫酸吲哚醇显著影响肠道稳态、免疫反应,并诱导全身促炎状态,这种刺激导致免疫系统产生促炎性介质[21]。壳寡糖可以通过下调丝裂原活化蛋白激酶(mitogen-activated protein kinase,MAPK)、Toll样受体4(Toll-like receptor 4,TLR4)等信号通路的磷酸化水平,减少核因子-κB抑制因子α(inhibitor of nuclear factor-κB α,IκBα)降解和细胞中核因子-κB(nuclear factor-κB,NF-κB)激活,抑制促炎细胞因子释放,发挥抗炎功能[22-23]。Youssef等[24]报道,壳寡糖能够提高肉鸡血清免疫球蛋白G(immunoglobulin G,IgG)和免疫球蛋白M(immunoglobulin M,IgM)含量。Chen等[25]报道,壳寡糖会激活巨噬细胞产生白细胞介素-6(interleukin 6,IL-6)和肿瘤坏死因子-α(tumor necrosis factor-α,TNF-α),提高白细胞和巨噬细胞活力,发挥抗炎作用。Lan等[26]研究表明,壳寡糖能降低热应激肉鸡肝脏白细胞介素-1β(interleukin-1β,IL-1β)和IL-6的表达,提高抗炎因子白细胞介素-10(interleukin-10,IL-10)的表达。

1.2.3 抗菌功能

壳寡糖不仅能抑制有害菌,例如大肠杆菌、金黄色葡萄球菌、假单胞菌及希瓦氏菌的数量,还能促进有益菌例如乳酸杆菌和双歧杆菌增殖[27-28]。壳寡糖还能抑制部分真菌例如白色念珠菌、热带念珠菌的生长[29-30]。壳寡糖通过带正电荷的氨基与带负电荷的微生物细胞壁结合,改变细菌细胞膜通透性致死有害菌,达到抑制细菌繁殖效果,壳寡糖抑菌性与其浓度、脱乙酰度和分子质量相关[31-32]。乙酰化能有效地抑制微生物生长,但脱乙酰化越高,分子质量越高,其中存在的大量游离氨基就会产生排斥力,从而减少与细菌细胞壁的相互作用,降低抗菌效果[29]

1.2.4 其他生物学功能

壳寡糖可以调节脂肪代谢,减少脂肪沉积。Wang等[33]报道,2 400和3 600 u壳寡糖能有效减少肝脏和腹部脂肪沉积,促进肝脏脂肪分解代谢。壳寡糖还对肿瘤增殖及转移有抑制效果[34]。Zou等[35]报道,每2 d腹腔注射1次40 mg/kg BW壳寡糖会诱导小鼠细胞凋亡抑制结肠癌HCT116细胞生长。壳寡糖还能作为药物载体,实现对肿瘤靶向,提高抗癌药物疗效[36]。Chen等[37]报道,基于壳寡糖制造的肿瘤靶向药物可以靶向肿瘤细胞表面受体,并针对特定肿瘤微环境释放药物,且抗肿瘤活性优于游离药物。

2 壳寡糖对肠道黏膜屏障的保护作用

2.1 壳寡糖对肠道黏膜微生物屏障的保护作用

肠道厌氧菌能减少病原微生物对黏膜的附着,增强肠黏膜屏障功能,是肠道黏膜重要的生物屏障[38-39]。肠道厌氧菌数量减少会导致肠道微生态失衡,破坏菌群稳定性,肠道生物屏障受损。肠道微生物种类越丰富,对有害刺激的抵抗力越强,调节肠道免疫功能的能力越强[40]。肠道中变形菌门(Proteobacteria)的富集代表不稳定微生物群落结构或宿主的疾病状态[41]。厚壁菌门(Firmicutes)菌群是正常菌群重要组成部分[42]。经黏液真杆菌属(Blautia)是一种共生专性厌氧菌属,在维持肠道环境平衡和预防炎症方面发挥重要作用[43]。双歧杆菌属(Bifidobacterium)菌群通过代谢活动为其宿主带来积极的健康益处[44]。志贺氏菌属(Shigella)是一类革兰阴性短小杆菌,能引起细菌性痢疾或志贺氏菌病[45]
壳寡糖对肠道黏膜微生物屏障功能的影响见表1。Na等[46]报道,壳寡糖能提高肠道厚壁菌门的相对丰度。张冉等[47]报道,壳寡糖能够降低小鼠肠道变形菌门和志贺氏菌属的相对丰度,提高厚壁菌门、双歧杆菌属和经黏液真杆菌属的相对丰度。王共旭[48]报道,壳寡糖会提高白羽王鸽回肠变形菌门的相对丰度,降低回肠厚壁菌门的相对丰度。Song等[49]报道,壳寡糖能改善热应激导致的肉鸡肠道乳酸菌和双歧杆菌的减少以及大肠杆菌和梭状芽胞杆菌的增加。施斐等[50]报道,壳寡糖会提高虎龙斑的生长性能,提高免疫力,改善肠道菌群及增强抗病力。以上研究表明,壳寡糖能改变肠道微生物群落的丰富度和多样性,增加有益菌数量的同时减少有害菌数量,缓解应激导致的肠道微生态失衡。
表1 壳寡糖对肠道黏膜微生物屏障功能的影响

Table 1 Effects of chitosan oligosaccharides on intestinal mucosal microbial barrier function

试验对象
Experimental
objects
壳寡糖属性
Chitosan
oligosaccharide
properties
添加量
Addition
amount
结果
Results
参考文献
References
1%葡聚糖硫酸钠诱导
结肠炎的C57BL/6小鼠
Colitis induced by 1% dextran
sulfate in C57BL/6 mice
分子质量1.78 ku,
脱乙酰度≥95%,
纯度94.4%
0.2 mg/mL
溶于磷酸
盐缓冲液
提高厚壁菌门
相对丰度
[46]
小鼠Mice 降低变形菌门和志贺氏菌属相对
丰度,提高厚壁菌门、经黏液
真杆菌属和双歧杆菌属相对丰度
[47]
白羽王鸽
White feather
royal pigeons
分子质量<3 ku,
纯度>85%
100、200和
400 mg/kg
提高回肠变形杆菌门相对丰度,
降低回肠厚壁菌门和拟杆
菌门相对丰度
[48]
热应激罗斯308肉鸡
Ross 308 broilers
under heat stress
脱乙酰
度>80%
1.5 g/kg 改善热应激导致的乳酸菌和双歧杆菌
数量的减少以及大肠杆菌和梭状
芽孢杆菌数量的增加
[49]
虎龙斑
Tiger dragon plaque
800 mg/kg 提高益生菌相对丰度 [50]

2.2 壳寡糖对肠道黏膜化学屏障的保护作用

化学屏障包括肠道黏膜上皮细胞分泌的消化酶、黏液以及肠道菌群产生的抑菌物质和短链脂肪酸等化学物质[51]。杯状细胞会分泌黏液覆盖于黏膜表面,黏液层能防止细菌与上皮细胞接触,且黏液中富含黏蛋白,此类蛋白会形成保护性黏液层,覆盖于上皮细胞表面,所以肠壁中杯状细胞数量能反映肠道产生黏蛋白的潜力[52]。动物肠道上皮细胞可产生大量抗菌肽(antimicrobial peptides,AMPs),其中最多的是防御素[53]
壳寡糖对肠道黏膜化学屏障功能的影响见表2。Xiong等[54]报道,30 mg/kg壳寡糖可以调控肠道黏液的产生,提高断奶仔猪回肠杯状细胞数量,这可能有助于其肠道保护作用。Wang等[55]报道,培养基中添加200 μg/mL壳寡糖能通过促进人结肠癌细胞的黏蛋白2(mucin 2,MUC2)表达,减轻硫酸葡聚糖钠诱导的损伤。Tao等[56]报道,壳寡糖能改善内毒素刺激下MUC2在空肠和结肠中的表达。Chen等[11]报道,壳寡糖能引起蛋白酶活化受体2(protease-activated receptor 2,PAR2),并促进与天然防御相关的β-防御素表达。Wei等[57]报道,壳寡糖能提高大鼠结肠中乙酸含量。Mohyuddin等[58]报道,壳寡糖能提高热应激小鼠的结肠黏液层厚度,增加杯状细胞的数量。以上研究表明,应激会减少动物黏蛋白含量,破坏肠道黏膜化学屏障功能。壳寡糖可以上调黏蛋白和杯状细胞的数量,促进短链脂肪酸的合成,促进防御素分泌,增加黏液层的厚度,维持肠道黏膜化学屏障功能。
表2 壳寡糖对肠道黏膜化学屏障功能的影响

Table 2 Effects of chitosan oligosaccharides on intestinal mucosal chemical barrier function

试验对象
Experimental
objects
壳寡糖属性
Chitosan
oligosaccharide
properties
添加量
Addition
amount
结果
Results
参考文献
References
断奶应激三元杂交仔猪
Three hybrid piglets with
weaning stress
分子质量1~2 ku 30 mg/kg 提高回肠杯状细胞数量 [54]
2%葡聚糖硫酸钠诱导的
人结肠癌细胞
2% glucan sulfate sodium
induced human colon cancer cells
分子质量363~
1 329 ku,脱
乙酰度>95%
200 μg/mL 促进结肠癌细胞黏蛋
白2(MUC2)表达
[55]
内毒素诱导肠道损伤的
C57BL/6小鼠
Endotoxin-induced intestinal
damage in C57BL/6 mice
400 mg/kg 改善MUC2在空肠和
结肠中的表达
[56]
内毒素诱导结肠炎的SD大鼠
Endotoxin-induced
colitis in SD rats
分子质
量<2 ku
45 mg/kg 提高结肠中乙酸含量 [57]
热应激小鼠
Heat stressed mice
分子质量<1 ku,
脱乙酰度>90%
300、
600 mg/kg
改善结肠黏液层厚度的降低以及
杯状细胞数量的减少
[58]

2.3 壳寡糖对肠道黏膜机械屏障的保护作用

肠道黏膜机械屏障由肠道黏膜上皮细胞和相邻细胞间连接等构成,肠上皮细胞包含吸收细胞、潘氏细胞等,相邻细胞间连接包括紧密连接(tight junction,TJ)、缝隙连接(gap junction,GJ)、黏附连接(adhesion junction,AJ)及桥粒连接(desmosome)[59-60]。壳寡糖可以减缓应激导致的肠道上皮细胞损伤,维持肠道黏膜机械屏障功能[61]。壳寡糖对肠道形态的影响见表3。Osho等[62]报道,饲粮添加1 g/kg壳寡糖能够有效缓解地塞米松诱导的肉鸡空肠绒毛高度降低及隐窝深度升高。Lan等[63]报道,壳寡糖能提高热应激肉鸡十二指肠、空肠和回肠的绒毛高度。Khambualai等[64]报道,饲粮添加0.6 g/kg壳寡糖能够增加肉鸡回肠绒毛面积和十二指肠细胞有丝分裂。Wan等[65]报道,壳寡糖能提高断奶应激仔猪十二指肠绒毛高度。Mohyuddin等[58]报道,壳寡糖能改善热应激导致的小鼠结肠长度和绒毛高度降低。Shi等[66]报道,壳寡糖可以通过提高罗非鱼肠道的肠壁厚度,改变肠道形态。以上研究表明,应激会降低动物肠道的绒毛高度,加深隐窝深度,破坏肠道机械屏障功能。壳寡糖能够有效减缓应激导致的肠道上皮细胞损伤,提高绒毛高度,降低隐窝深度,提高肠壁厚度,维持肠道黏膜机械屏障功能。
表3 壳寡糖对肠道形态的影响

Table 3 Effects of chitosan oligosaccharides on intestinal morphology

试验对象
Experimental
objects
壳寡糖属性
Chitosan
oligosaccharide
properties
添加量
Addition
amount
结果
Results
参考文献
References
地塞米松诱导应激
科宝500肉鸡
Dexamethasone induced
stress in Cobb 500 broilers
脱乙酰度
>90%
1 g/kg 缓解空肠绒毛高度降低及隐窝
深度升高,提高回肠消化率
[62]
热应激黄羽肉鸡
Yellow feather broilers
under heat stress
分子质量
≤3.2 ku
200 mg/kg 改善十二指肠、空肠和
回肠绒毛高度的降低
[63]
马歇尔矮胖肉鸡
Marshall chunky broilers
脱乙酰度
90%
0.6 g/kg 回肠绒毛面积和十二指肠
细胞有丝分裂增加
[64]
断奶应激长白×约克猪
Landrace×Yorkshire pigs
with weaning stress
100 mg/kg 提高十二指肠绒毛高度 [65]
热应激小鼠
Heat stressed mice
分子质量
<1 ku,脱乙
酰度>90%
300、
600 mg/kg
改善结肠长度和
绒毛高度降低
[58]
罗非鱼Tilapia 400 mg/kg 提高肠道肠壁厚度 [66]
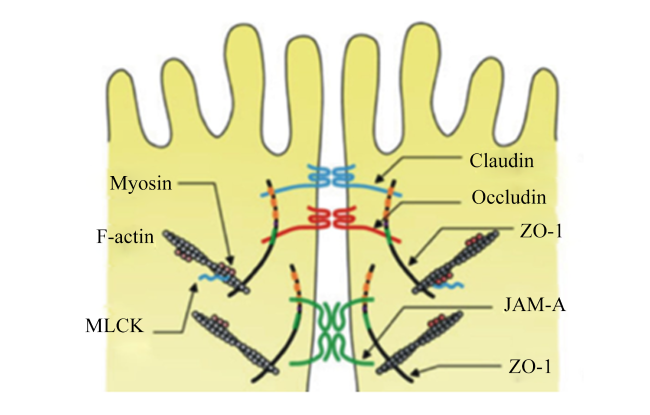
细胞间连接由紧密连接、黏附连接、间隙连接和桥粒连接组成,其中紧密连接具有维持肠道黏膜机械屏障完整性的功能,是肠上皮细胞间的核心[67]。紧密连接(图2)由闭合蛋白(occludin)、封闭蛋白(claudin)和连接黏附分子(junctional adhesion molecule,JAM)等跨膜蛋白,闭锁小带蛋白(zonula occludens,ZO)等胞质蛋白,以及细胞骨架构成紧密连接复合物[68]。跨膜蛋白可通过胞质蛋白与细胞骨架联系在一起[69]。壳寡糖对肠道黏膜紧密链接屏障功能的影响见表4。Li等[70]报道,壳寡糖会上调肉鸡空肠和回肠claudin-3的mRNA表达。Osho等[62]报道,饲粮添加1 g/kg壳寡糖能够提高地塞米松应激肉鸡肠道occludin和claudin-1的mRNA表达。Osho等[71]报道,饲粮添加1 g/kg壳寡糖可以提高球虫攻毒肉鸡肠道ZO-1、ZO-2、claudin-1和occludin的mRNA表达。Wang等[55]报道,培养基添加200 μg/mL壳寡糖能减轻硫酸葡聚糖钠诱导的人结肠癌细胞损伤,提高occludin的表达。Shi等[72]报道,壳寡糖能提高猪肠上皮细胞跨膜电阻(trans-epithelial electrical resistance,TEER)值。Pinton等[73]报道,激活MAPK信号通路中的细胞外信号调节激酶(extracellular signal-regulated kinase,ERK)是破坏肠道黏膜机械屏障完整性的作用机制。Luo等[74]报道,壳寡糖可以抑制p38 MAPK和ERK磷酸化的增加,保护因为氧化应激而损伤的细胞。施斐等[50]报道,饲粮添加400和800 mg/kg壳寡糖会提高虎龙斑肠道ZO-1、ZO-2、ZO-3和claudin-3α的mRNA表达量。以上研究表明,应激会降低肠道细胞存活率,通过降低紧密连接蛋白表达量增强肠上皮通透性,从而损伤肠道机械屏障功能。壳寡糖能够有效减缓应激导致的肠道上皮细胞损伤、提高紧密连接蛋白表达量增加肠道通透性,维持肠道黏膜机械屏障功能。
图2 紧密连接屏障

Myosin:肌球蛋白;F-actin:丝状肌动蛋白 filamentous actin;MLCK:肌球蛋白轻链激酶 myosin light-chain kinase;Claudin:封闭蛋白;Occludin:闭合蛋白;ZO-1:闭锁小带蛋白-1 zonula occludens-1;JAM-A:连接黏附分子-A junctional adhesion molecule-A。

Fig.2 Tight junction barrier[68]

表4 壳寡糖对肠道黏膜紧密连接屏障功能的影响

Table 4 Effects of chitosan oligosaccharides on intestinal mucosal tight junction barrier function

试验对象
Experimental
objects
壳寡糖属性
Chitosan
oligosaccharide
properties
添加量
Addition
amount
结果
Results
参考文献
References
爱拔益加肉鸡
Arbor Acres broilers
分子质量1~2 ku,
脱乙酰度>90%
30 mg/kg 上调空肠和回肠
claudin-3的mRNA表达
[70]
地塞米松诱导应激科宝500肉鸡
Dexamethasone induced
stress in Cobb 500 broilers
脱乙酰
度>90%
1 g/kg 提高空肠occludin和
claudin-1的mRNA表达量
[62]
球虫疫苗诱导应激科宝500肉鸡
Coccidia vaccine induced stress in
Cobb 500 broilers
脱乙酰
度>90%
1 g/kg 提高ZO-1、ZO-2、claudin-1
和occludin的mRNA表达量
[71]
乙醇诱导应激人L02肝细胞
Ethanol induced stress in
human L02 hepatocytes
分子质量
<1 ku,脱乙
酰度≥95%
0.25、0.50、
1.00 mg/mL
抑制p38 MAPK和
ERK磷酸化增加
[74]
2%葡聚糖硫酸钠诱导人结肠癌细胞
2% sodium dextran sulfate induced
human colon cancer cells
分子质量
363~1 329 ku,
脱乙酰度>95%
200 μg/mL 提高occludin的表达量 [55]
内毒素诱导应激猪肠上皮细胞
Endotoxin induced stress in
porcine intestinal epithelial cells
分子质量
<1 ku,脱乙
酰度90%
200、
800 μg/mL
提高细胞存活率和TEER值 [72]
虎龙斑
Tiger dragon plaque
400、
800 mg/kg
提高肠道ZO-1、ZO-2、ZO-3和
claudin-3α的mRNA表达量
[50]

claudin:封闭蛋白;occludin:闭合蛋白;ZO:闭锁小带蛋白 zonula occludens;MAPK:丝裂原活化蛋白激酶 mitogen-activated protein kinase;ERK:细胞外信号调节激酶 extracellular signal-regulated kinase;TEER:上皮细胞跨膜电阻 trans-epithelial electrical resistance。

2.4 壳寡糖对肠道黏膜免疫屏障的保护作用

肠道黏膜免疫屏障由肠道浆细胞、肠系膜淋巴结、肠道相关淋巴组织(gut associated lymphatic tissue,GALT)构成[8]。其中,肠道淋巴细胞分泌的分泌型免疫球蛋白A(secretory immunoglobulin A,sIgA)可以刺激肠道黏液分泌,阻止病原体在黏膜表面黏附,与细菌毒素中和,抑制细菌增殖[75]。肠道中sIgA减少会导致肠道免疫屏障功能下降,增加黏膜上皮细胞对于肠道细菌产生的内毒素的吸收[76]。免疫球蛋白A(immunoglobulin A,IgA)是胃肠道主要抗体同种型,在黏膜分泌物中以sIgA多反应性二聚体的形式易位,并保护肠上皮免受毒素和病原微生物的侵害[77]。IgM是体内免疫反应发生时最先出现的抗体,出现后迅速激活B细胞,产生其他免疫球蛋白。IgG是免疫应答所产生的主要抗体,在免疫过程中起到抗菌、中和病毒及免疫调节的重要作用,IgG含量降低会导致肠道免疫反应失衡,从而破坏肠道黏膜免疫屏障[78]
当肠道黏膜免疫功能被破坏后,黏膜受到细菌等抗原刺激,导致淋巴细胞产生IL-1β、IL-6、白细胞介素-8(interleukin-8,IL-8)、TNF-α、干扰素-γ(interferon-γ,IFN-γ)等促炎细胞因子以及IL-10等抗炎细胞因子。促炎细胞因子水平越高,全身炎症反应越重,抗炎细胞因子则相反[12]。壳寡糖对肠道黏膜免疫屏障功能的影响见表5。Gu等[79]报道,壳寡糖可以改善内毒素导致的海兰褐壳蛋鸡回肠和空肠sIgA、IgG、IgM含量升高,降低空肠和回肠IL-1β和IFN-γ含量。Lan等[63]报道,壳寡糖可以缓解热应激导致的黄羽肉鸡十二指肠和空肠黏膜IL-1β含量升高。Osho等[62]报道,壳寡糖可以缓解科宝500肉鸡地塞米松应激,降低空肠IL-6含量,提高IL-10含量,并降低IL-8和TNF-α的mRNA表达量。Xiong等[54]报道,壳寡糖能增加断奶仔猪十二指肠和空肠上皮内淋巴细胞数量,但会减少回肠上皮内淋巴细胞数量。Shi等[72]报道,壳寡糖能缓解内毒素应激的猪肠上皮细胞损伤,降低IL-6和IL-8的mRNA表达量。以上研究结果表明,应激会导致肠道sIgA、IgG、IgM含量升高,淋巴细胞增加,促炎细胞因子分泌,破坏肠道免疫屏障功能。壳寡糖有抗炎作用,减少促炎细胞因子分泌,提高抗炎细胞因子分泌,降低肠道的通透性,维持肠道黏膜免疫屏障功能。
表5 壳寡糖对肠道黏膜免疫屏障功能的影响

Table 5 Effects of chitosan oligosaccharides on intestinal mucosal immune barrier function

试验对象
Experimental
objects
壳寡糖属性
Chitosan
oligosaccharide
properties
添加量
Addition
amount
结果
Results
参考文献
References
断奶应激三元杂交仔猪
Three hybrid piglets with
weaning stress
分子质量
1~2 ku
30 mg/kg 增加十二指肠和空肠淋巴
细胞数量,减少回肠淋巴细胞数量
[54]
地塞米松诱导应激科宝500肉鸡
Dexamethasone induced stress
in Cobb 500 broilers
脱乙酰
度>90%
1 g/kg 降低空肠IL-6含量,提高IL-10
含量,降低IL-8、TNF-α
mRNA表达量
[62]
热应激黄羽肉鸡
Yellow feather broilers
under heat stress
分子质量
<32 ku,脱乙
酰度>95%
200 mg/kg 降低十二指肠和
空肠黏膜IL-1β含量
[63]
内毒素诱导应激猪肠上皮细胞
Endotoxin induced stress in
porcine intestinal epithelial cells
分子质量
<1 ku,脱乙
酰度90%
200 μg/mL 降低IL-6和IL-8
的mRNA表达量
[72]
内毒素诱导应激海兰褐壳蛋鸡
Endotoxin induced stress in
Hy-Line brown laying hens
分子质量
1~2 ku,脱
乙酰度90%
15 mg/kg 降低回肠和空肠sIgA、IgG、
IgM、IL-1β和IFN-γ含量
[79]

IL:白细胞介素 interleukin;TNF-α:肿瘤坏死因子-α tumor necrosis factor-α;sIgA:分泌型免疫球蛋白A secretory immunoglobulin A;IgG:免疫球蛋白G immunoglobulin G;IgM:免疫球蛋白M immunoglobulin M;IFN-γ:干扰素-γ interferon-γ。

3 小结与展望

综上所述,目前关于壳寡糖对肠道黏膜屏障功能保护的研究在单胃动物中已有一定成果,但对其作用机制的深入探讨,特别是相关信号通路的研究尚不够充分。鉴于此,未来针对壳寡糖对肠道黏膜屏障保护效应的研究工作,建议应着重从以下几个方面进行拓展:1)加强对单胃动物体内壳寡糖影响肠道黏膜屏障完整性的具体信号通路的探索,并进一步将研究范围扩大至反刍动物,以填补该领域在反刍动物体内的研究空白,全面解析壳寡糖在不同消化生理特征动物中的肠道屏障保护作用及其分子机制;2)研究壳寡糖在动物生产中最适宜的种类、添加量、去乙酰化程度、聚合度和纯度等;3)研究壳寡糖对于不同肠段和肠道屏障的保护作用及其机理。
[1]
WANG L L, WANG C N, PENG Y, et al. Research progress on anti-stress nutrition strategies in swine[J]. Animal Nutrition, 2023,13:342-360.

[2]
SAEED M, ABBAS G, ALAGAWANY M, et al. Heat stress management in poultry farms:a comprehensive overview[J]. Journal of Thermal Biology, 2019,84:414-425.

[3]
ABD EL-HACK M E, EL-SAADONY M T, SHAFI M E, et al. Antimicrobial and antioxidant properties of chitosan and its derivatives and their applications:a review[J]. International Journal of Biological Macromolecules, 2020,164:2726-2744.

[4]
LIU W, LI X Q, ZHAO Z L, et al. Effect of chitooligosaccharides on human gut microbiota and antiglycation[J]. Carbohydrate Polymers, 2020,242:116413.

[5]
WANG Y K, ZHU H B, WANG X J, et al. Natural food polysaccharides ameliorate inflammatory bowel disease and its mechanisms[J]. Foods, 2021, 10(6):1288.

[6]
ANIL S. Potential medical applications of chitooligosaccharides[J]. Polymers, 2022, 14(17):3558.

[7]
HOROWITZ A, CHANEZ-PAREDES S D, HAEST X, et al. Paracellular permeability and tight junction regulation in gut health and disease[J]. Nature Reviews:Gastroenterology & Hepatology, 2023, 20(7):417-432.

[8]
高亚男, 王加启, 李松励, 等. 霉菌毒素影响肠道黏膜屏障功能[J]. 动物营养学报, 2016, 28(3):674-679.

GAO Y N, WANG J Q, LI S L, et al. Effects of mycotoxins on intestinal mucosal barrier function[J]. Chinese Journal of Animal Nutrition, 2016, 28(3):674-679. (in Chinese)

[9]
SADURNÍ M, BARROETA A C, SOL C, et al. Short communication:evaluation of intestinal release of butyric acid from sodium butyrate protected by salts of medium-chain fatty acids in broiler chickens[J]. Animals, 2022, 12(24):3525.

[10]
CHEN Y L, LING Z M, WANG X, et al. The beneficial mechanism of chitosan and chitooligosaccharides in the intestine on different health status[J]. Journal of Functional Foods, 2022,97:105232.

[11]
CHEN C L, WANG Y M, LIU C F, et al. The effect of water-soluble chitosan on macrophage activation and the attenuation of mite allergen-induced airway inflammation[J]. Biomaterials, 2008, 29(14):2173-2182.

[12]
KUSHIBIKI S. Tumor necrosis factor-α-induced inflammatory responses in cattle[J]. Animal Science Journal, 2011, 82(4):504-511.

DOI PMID

[13]
WEN J Y, CHEN S W, BAO M L, et al. Slc9a1 plays a vital role in chitosan oligosaccharide transport across the intestinal mucosa of mice[J]. Carbohydrate Polymers, 2023,299:120179.

[14]
LIANG S, SUN Y X, DAI X L. A review of the preparation,analysis and biological functions of chitooligosaccharide[J]. International Journal of Molecular Sciences, 2018, 19(8):2197.

[15]
EMAMI N K, JUNG U, VOY B, et al. Radical response:effects of heat stress-induced oxidative stress on lipid metabolism in the avian liver[J]. Antioxidants, 2020, 10(1):35.

[16]
YANG L, WAN Y, LI W W, et al. Targeting intestinal flora and its metabolism to explore the laxative effects of rhubarb[J]. Applied Microbiology and Biotechnology, 2022, 106(4):1615-1631.

DOI PMID

[17]
LIAQAT F, ELTEM R. Chitooligosaccharides and their biological activities:a comprehensive review[J]. Carbohydrate Polymers, 2018,184:243-259.

[18]
何雪萍. 不同分子量壳寡糖对黄羽肉鸡生长、抗氧化及免疫功能的影响[D]. 硕士学位论文. 湛江: 广东海洋大学, 2022.

HE X P. Effects of different molecular weight chito-oligosaccharides on growth,antioxidant and immune function of yellow-feathered broilers[D]. Master’s Thesis. Zhenjiang: Guangdong Ocean University, 2022. (in Chinese)

[19]
XU Q Q, AZZAM M M M, ZOU X T, et al. Effects of chitooligosaccharide supplementation on laying performance,egg quality,blood biochemistry,antioxidant capacity and immunity of laying hens during the late laying period[J]. Italian Journal of Animal Science, 2020, 19(1):1180-1187.

[20]
LAN R, CHEN X, ZHANG Y, et al. Effects of dietary chitosan oligosaccharides supplementation on meat quality,chemical composition and anti-oxidant capacity in frizzled chickens[J]. Italian Journal of Animal Science, 2023, 22(1):639-650.

[21]
RAPA S F, PRISCO F, POPOLO A, et al. Pro-inflammatory effects of indoxyl sulfate in mice:impairment of intestinal homeostasis and immune response[J]. International Journal of Molecular Sciences, 2021, 22(3):1135.

[22]
KIM J H, KIM Y S, HWANG J W, et al. Sulfated chitosan oligosaccharides suppress LPS-induced NO production via JNK and NF-κB inactivation[J]. Molecules, 2014, 19(11):18232-18247.

[23]
FENG J Y, LIU Y J, CHEN J J, et al. Marine chitooligosaccharide alters intestinal flora structure and regulates hepatic inflammatory response to influence nonalcoholic fatty liver disease[J]. Marine Drugs, 2022, 20(6):383.

[24]
YOUSSEF I M, KHALIL H A, SHAKOORI A M, et al. Immune response,hematological traits,biochemical blood parameters,and histological status of laying hens influenced by dietary chitosan-oligosaccharides[J]. Poultry Science, 2023, 102(9):102834.

[25]
CHEN J J, YANG Y C, XU Z Z, et al. Characterization of effects of chitooligosaccharide monomer addition on immunomodulatory activity in macrophages[J]. Food Research International, 2023,163:112268.

[26]
LAN R X, LUO H W, WU F, et al. Chitosan oligosaccharides alleviate heat-stress-induced lipid metabolism disorders by suppressing the oxidative stress and inflammatory response in the liver of broilers[J]. Antioxidants, 2023, 12(8):1497.

[27]
KE C L, DENG F S, CHUANG C Y, et al. Antimicrobial actions and applications of chitosan[J]. Polymers, 2021, 13(6):904.

[28]
罗威, 黄晓月, 钟萍, 等. 不同分子质量虾源壳寡糖的抗菌抗氧化活性差异研究[J]. 食品与发酵工业, 2023, 49(24):193-197.

DOI

LUO W, HUANG X Y, ZHONG P, et al. Antibacterial and antioxidant activities of shrimp-derived chitosan oligosaccharides with different molecular weights[J]. Food and Fermentation Industries, 2023, 49(24):193-197. (in Chinese)

DOI

[29]
ING L Y, ZIN N M, SARWAR A, et al. Antifungal activity of chitosan nanoparticles and correlation with their physical properties[J]. International Journal of Biomaterials, 2012,2012:632698.

[30]
ALBURQUENQUE C, BUCAREY S A, NEIRA-CARRILLO A, et al. Antifungal activity of low molecular weight chitosan against clinical isolates of Candida spp[J]. Medical Mycology, 2010, 48(8):1018-1023.

[31]
YIN N, DU R P, ZHAO F K, et al. Characterization of antibacterial bacterial cellulose composite membranes modified with chitosan or chitooligosaccharide[J]. Carbohydrate Polymers, 2020,229:115520.

[32]
SÁNCHEZ Á, MENGÍBAR M, RIVERA-RODRÍGUEZ G, et al. The effect of preparation processes on the physicochemical characteristics and antibacterial activity of chitooligosaccharides[J]. Carbohydrate Polymers, 2017,157:251-257.

[33]
WANG R L, CHEN J W, GOONERATNE R, et al. Effects of varied molecular weight of chitosan oligosaccharides on growth performance,carcass trait,meat quality,and fat metabolism in indigenous yellow-feathered chickens[J]. Journal of Applied Poultry Research, 2022, 31(1):100221.

[34]
ZHAI X C, LI C N, REN D F, et al. The impact of chitooligosaccharides and their derivatives on the in vitro and in vivo antitumor activity:a comprehensive review[J]. Carbohydrate Polymers, 2021,266:118132.

[35]
ZOU P, YUAN S J, YANG X, et al. Chitosan oligosaccharides with degree of polymerization 2-6 induces apoptosis in human colon carcinoma HCT116 cells[J]. Chemico-Biological Interactions, 2018,279:129-135.

[36]
YU D W, FENG J Y, YOU H M, et al. The microstructure,antibacterial and antitumor activities of chitosan oligosaccharides and derivatives[J]. Marine Drugs, 2022, 20(1):69.

[37]
CHEN X, BREMNER D H, YE Y H, et al. A dual-prodrug nanoparticle based on chitosan oligosaccharide for enhanced tumor-targeted drug delivery[J]. Colloids and Surfaces A:Physicochemical and Engineering Aspects, 2021,619:126512.

[38]
GUO S W, XING Y Y, XU Y Q, et al. Progress of studies on plant-derived polysaccharides affecting intestinal barrier function in poultry[J]. Animals, 2022, 12(22):3205.

[39]
WALSH A M, SWEENEY T, BAHAR B, et al. The effect of chitooligosaccharide supplementation on intestinal morphology,selected microbial populations,volatile fatty acid concentrations and immune gene expression in the weaned pig[J]. Animal, 2012, 6(10):1620-1626.

[40]
VON MARTELS J Z H, SADAGHIAN SADABAD M, BOURGONJE A R, et al. The role of gut microbiota in health and disease:in vitro modeling of host-microbe interactions at the aerobe-anaerobe interphase of the human gut[J]. Anaerobe, 2017,44:3-12.

[41]
SHIN N R, WHON T W, BAE J W. Proteobacteria:microbial signature of dysbiosis in gut microbiota[J]. Trends in Biotechnology, 2015, 33(9):496-503.

[42]
CHEN T Y, DING R R, CHEN X R, et al. Firmicutes and Blautia in gut microbiota lessened in chronic liver diseases and hepatocellular carcinoma patients:a pilot study[J]. Bioengineered, 2021, 12(1):8233-8246.

[43]
HOSOMI K, SAITO M, PARK J, et al. Oral administration of Blautia wexlerae ameliorates obesity and type 2 diabetes via metabolic remodeling of the gut microbiota[J]. Nature Communications, 2022, 13(1):4477.

[44]
O’CALLAGHAN A, VAN SINDEREN D. Bifidobacteria and their role as members of the human gut microbiota[J]. Frontiers in Microbiology, 2016,7:925.

[45]
KIM Y I, YANG J Y, KO H J, et al. Shigella flexneri inhibits intestinal inflammation by modulation of host sphingosine-1-phosphate in Mice[J]. Immune Network, 2014, 14(2):100-106.

[46]
NA K, WEI J N, ZHANG L, et al. Effects of chitosan oligosaccharides (COS) and FMT from COS-dosed mice on intestinal barrier function and cell apoptosis[J]. Carbohydrate Polymers, 2022,297:120043.

[47]
张冉, 唐余燕, 贺海东, 等. 壳寡糖通过调控肠道微生态及IgA免疫系统对IgA肾病的改善作用研究[C]// 中国食品科学技术学会第十九届年会. 合肥: 中国食品科学技术学会,2022:148-149.

ZHANG R, TANG Y Y, HE H D, et al. Amelioration effects of chitooligosaccharides on IgA nephropathy through regulation of intestinal microbiology and IgA immune system[C]// The 19th Annual Meeting of Chinese Society of Food Science and Technology. Hefei: Chinese Society of Food Science and Technology,2022:148-149. (in Chinese)

[48]
王共旭. 日粮中添加壳寡糖对白羽王鸽免疫性能、抗氧化性能及肠道发育的影响[D]. 硕士学位论文. 乌鲁木齐: 新疆农业大学, 2022.

WANG G X. Effects of dietary chitosan oligosaccharides on immune performance,antioxidant performance and intestinal development of white feather royal pigeon[D]. Master’s Thesis. Urumqi: Xinjiang Agricultural University, 2022. (in Chinese)

[49]
SONG J, JIAO L F, XIAO K, et al. Cello-oligosaccharide ameliorates heat stress-induced impairment of intestinal microflora,morphology and barrier integrity in broilers[J]. Animal Feed Science and Technology, 2013, 185(3/4):175-181.

[50]
施斐, 黄垚, 卢志杰, 等. 壳寡糖对虎龙斑的生长、免疫及肠道菌群的影响[J]. 水产学报, 2022, 46(9):1689-1700.

SHI F, HUANG Y, LU Z J, et al. Effects of chito-oligosaccharides on the growth,immunity and intestinal flora of the tiger dragon plaque[J]. Journal of Fisheries of China, 2022, 46(9):1689-1700. (in Chinese)

[51]
HAO W D, HAO C Y, WU C R, et al. Aluminum induced intestinal dysfunction via mechanical,immune,chemical and biological barriers[J]. Chemosphere, 2022,288:132556.

[52]
王涛, 田欣蕾, 张迪, 等. 益生菌调节肠道黏膜免疫研究进展[J]. 中国兽医学报, 2022, 42(12):2578-2584.

WANG T, TIAN X L, ZHANG D, et al. Research progress in probiotic bacteria modulating intestinal mucosal immunity[J]. Chinese Journal of Veterinary Science, 2022, 42(12):2578-2584. (in Chinese)

[53]
SELSTED M E, MILLER S I, HENSCHEN A H, et al. Enteric defensins:antibiotic peptide components of intestinal host defense[J]. The Journal of Cell Biology, 1992, 118(4):929-936.

[54]
XIONG X, YANG H S, WANG X C, et al. Effect of low dosage of chito-oligosaccharide supplementation on intestinal morphology,immune response,antioxidant capacity,and barrier function in weaned piglets[J]. Journal of Animal Science, 2015, 93(3):1089-1097.

[55]
WANG Y J, WEN R, LIU D D, et al. Exploring effects of chitosan oligosaccharides on the DSS-induced intestinal barrier impairment in vitro and in vivo[J]. Molecules, 2021, 26(8):2199.

[56]
TAO W J, WANG G, PEI X, et al. Chitosan oligosaccharide attenuates lipopolysaccharide-induced intestinal barrier dysfunction through suppressing the inflammatory response and oxidative stress in mice[J]. Antioxidants, 2022, 11(7):1384.

[57]
WEI X J, YU L L, ZHANG C, et al. Prebiotic activity of chitooligosaccharides and their ability to alleviate necrotizing enterocolitis in newborn rats[J]. Carbohydrate Polymers, 2023,299:120156.

[58]
MOHYUDDIN S G, QAMAR A, HU C Y, et al. Effect of chitosan on blood profile,inflammatory cytokines by activating TLR4/NF-κB signaling pathway in intestine of heat stressed mice[J]. Scientific Reports, 2021, 11(1):20608.

[59]
DRABIÑSKA N, JAROCKA-CYRTA E. Crosstalk between resveratrol and gut barrier:a review[J]. International Journal of Molecular Sciences, 2022, 23(23):15279.

[60]
CHEN S S, ZHANG C, HE B H, et al. The role of lncRNAs in regulating the intestinal mucosal mechanical barrier[J]. BioMed Research International, 2021,2021:2294942.

[61]
陶文静. 壳寡糖对小鼠急性和慢性应激损伤的缓解作用及其机制研究[D]. 博士学位论文. 杭州: 浙江大学, 2020.

TAO W J. Study on the alleviating effect of chito-oligosaccharides on acute and chronic stress injury in mice and its mechanism[D]. Ph.D. Thesis. Hangzhou: Zhejiang University, 2020. (in Chinese)

[62]
OSHO S O, ADEOLA O. Chitosan oligosaccharide supplementation alleviates stress stimulated by in-feed dexamethasone in broiler chickens[J]. Poultry Science, 2020, 99(4):2061-2067.

DOI PMID

[63]
LAN R X, LI Y X, CHANG Q Q, et al. Dietary chitosan oligosaccharides alleviate heat stress-induced intestinal oxidative stress and inflammatory response in yellow-feather broilers[J]. Poultry Science, 2020, 99(12):6745-6752.

DOI PMID

[64]
KHAMBUALAI O, YAMAUCHI K, TANGTAWEEWIPAT S, et al. Growth performance and intestinal histology in broiler chickens fed with dietary chitosan[J]. British Poultry Science, 2009, 50(5):592-597.

DOI PMID

[65]
WAN J, JIANG F, XU Q, et al. New insights into the role of chitosan oligosaccharide in enhancing growth performance,antioxidant capacity,immunity and intestinal development of weaned pigs[J]. RSC Advances, 2017, 7(16):9669-9679.

[66]
SHI F, QIU X L, NIE L J, et al. Effects of oligochitosan on the growth,immune responses and gut microbes of tilapia (Oreochromis niloticus)[J]. Fish & Shellfish Immunology, 2020,106:563-573.

[67]
PARADIS T, BÈGUE H, BASMACIYAN L, et al. Tight junctions as a key for pathogens invasion in intestinal epithelial cells[J]. International Journal of Molecular Sciences, 2021, 22(5):2506.

[68]
SUZUKI T. Regulation of the intestinal barrier by nutrients:the role of tight junctions[J]. Animal Science Journal, 2020, 91(1):e13357.

[69]
杨雪, 高亚男, 王加启, 等. 霉菌毒素对肠道紧密连接蛋白的影响及其调控机制[J]. 动物营养学报, 2020, 32(12):5566-5577.

DOI

YANG X, GAO Y N, WANG J Q, et al. Effects of mycotoxin on intestinal tight junction protein and its regulation mechanism[J]. Chinese Journal of Animal Nutrition, 2020, 32(12):5566-5577. (in Chinese)

[70]
LI J, CHENG Y F, CHEN Y P, et al. Dietary chitooligosaccharide inclusion as an alternative to antibiotics improves intestinal morphology,barrier function,antioxidant capacity,and immunity of broilers at early age[J]. Animals, 2019, 9(8):493.

[71]
OSHO S O, ADEOLA O. Impact of dietary chitosan oligosaccharide and its effects on coccidia challenge in broiler chickens[J]. British Poultry Science, 2019, 60(6):766-776.

DOI PMID

[72]
SHI L, FANG B, YONG Y H, et al. Chitosan oligosaccharide-mediated attenuation of LPS-induced inflammation in IPEC-J2 cells is related to the TLR4/NF-κB signaling pathway[J]. Carbohydrate Polymers, 2019,219:269-279.

[73]
PINTON P, BRAICU C, NOUGAYREDE J P, et al. Deoxynivalenol impairs porcine intestinal barrier function and decreases the protein expression of claudin-4 through a mitogen-activated protein kinase-dependent mechanism[J]. The Journal of Nutrition, 2010, 140(11):1956-1962.

[74]
LUO Z G, DONG A A, KE Q, et al. Chitooligosaccharides inhibit ethanol-induced oxidative stress via activation of Nrf2 and reduction of MAPK phosphorylation[J]. Oncology Reports, 2014, 32(5):2215-2222.

DOI PMID

[75]
SEIKRIT C, PABST O. The immune landscape of IgA induction in the gut[J]. Seminars in Immunopathology, 2021, 43(5):627-637.

DOI PMID

[76]
CORTHÉSY B. Roundtrip ticket for secretory IgA:role in mucosal homeostasis?[J]. Journal of Immunology, 2007, 178(1):27-32.

[77]
NOVAL RIVAS M, WAKITA D, FRANKLIN M K, et al. Intestinal permeability and IgA provoke immune vasculitis linked to cardiovascular inflammation[J]. Immunity, 2019, 51(3):508-521.e6.

DOI PMID

[78]
CASTRO-DOPICO T, CLATWORTHY M R. IgG and Fcγ receptors in intestinal immunity and inflammation[J]. Frontiers in Immunology, 2019,10:805.

[79]
GU Y F, CHEN Y P, JIN R, et al. Dietary chitooligosaccharide supplementation alleviates intestinal barrier damage,and oxidative and immunological stress in lipopolysaccharide-challenged laying hens[J]. Poultry Science, 2022, 101(4):101701.

Outlines

/