REVIEW

Effects of Amino Acids, Glucose, Fatty Acids and Their Interactions on Milk Protein Synthesis

  • LIN Shaoxiong ,
  • SUN Mei ,
  • XING Yuanyuan ,
  • LI Dabiao , *
Expand
  • Inner Mongolia Key Laboratory of Animal Nutrition and Feed Science, College of Animal Science, Inner Mongolia Agricultural University, Hohhot 010018, China
*professor, E-mail:

Received date: 2024-05-10

  Online published: 2024-12-12

Abstract

Milk protein is the primary nutrient in milk. Its amino acid content and composition ratio closely match the needs of the human body. Additionally, it contains immunoglobulin, which is essential for newborn animals, making it an ideal source of protein. The mammary gland is the primary site for milk protein synthesis. It takes up nutrients, such as amino acids (AA), glucose (GLU), and fatty acids (FA), from the blood. These nutrients act as raw materials and energy substrates for milk protein synthesis, as well as signaling factors that regulate the synthesis of milk proteins. AA activates the mammalian target of rapamycin (mTOR), the activator of tyrosine kinase 2-signal transducer activator of transcription 5 (JAK2-STAT5), and the general regulatory inhibition of protein kinase 2 (GCN2) signaling pathways to regulate milk protein synthesis. On the other hand, GLU inhibits adenylate-activated protein kinase (AMPK) activity, upregulates the phosphorylation levels of downstream targets such as mTOR and ribosomal S6 protein kinase 1 (S6K1), and promotes milk protein synthesis. FA can mediate the AMPK signaling pathway to regulate intracellular FA synthesis and oxidation processes to meet the energy requirements for milk protein synthesis. This paper mainly summarizes the effects of AA, GLU and FA and their interactions on the synthesis of milk protein and its mechanism of action. It aims to explore the synthesis of milk protein and its mechanism of action from the perspective of the interaction of nutritional substrates, and to provide a theoretical reference for the regulation of milk protein synthesis by AA, GLU and FA.

Cite this article

LIN Shaoxiong , SUN Mei , XING Yuanyuan , LI Dabiao . Effects of Amino Acids, Glucose, Fatty Acids and Their Interactions on Milk Protein Synthesis[J]. Chinese Journal of Animal Nutrition, 2024 , 36(12) : 7553 -7562 . DOI: 10.12418/CJAN2024.643

牛奶中乳蛋白富含机体所需的必需氨基酸和易于吸收的蛋白质,被认为是理想的蛋白质来源[1]。在乳蛋白的合成过程中,大量的营养物质在胃肠道微生物和消化酶的作用下降解产生氨基酸(amino acids,AA)、葡萄糖(glucose,GLU)和脂肪酸(fatty acids,FA)等小分子化合物,然后被肠毛细血管吸收入血,经过血液循环运输至奶牛乳腺中,最后通过载体蛋白的转运进入乳腺细胞内,参与代谢途径中的能量产生和乳蛋白合成等过程[2]。研究表明,AA、GLU和FA作为乳蛋白合成的营养性底物,牛奶中约90%的乳蛋白是由血液中的游离AA合成,GLU和FA是奶牛泌乳和维持组织器官功能的能量底物,可以通过糖酵解和线粒体氧化等过程产生ATP,为乳蛋白的合成提供能量[3]。此外,AA、GLU和FA及其代谢产物还能够通过影响哺乳动物雷帕霉素靶蛋白(mammalian targets of rapamycin,mTOR)和腺苷酸活化蛋白激酶(AMP activated protein kinase,AMPK)等信号通路调节乳蛋白的合成[4]
近年来研究表明,相比于单一添加组,组合添加AA、GLU和FA可以显著促进奶牛乳腺上皮细胞(bovine mammary epithelial cells,BMECs)中乳蛋白合成相关基因和蛋白的表达,促进乳蛋白的合成。这说明营养性底物在乳蛋白合成过程中可能存在一种互作效应,可以最大限度促进乳蛋白的合成。但是,目前关于营养性底物互作调控乳蛋白合成的作用机制尚不清楚。因此,本文综述了AA、GLU和FA及其互作对乳蛋白合成的调控作用及其机理,旨在从营养性底物互作的角度为提高乳蛋白合成提供参考。

1 AA对牛奶乳蛋白合成的调控作用及其机理

1.1 AA供应调控牛奶乳蛋白合成

AA作为构成蛋白质的原料底物,其供应量直接影响牛奶中乳蛋白含量。Zhao等[5]研究发现,在奶牛低蛋白质饲粮中添加5 g/d过瘤胃蛋氨酸,可以显著提高产奶量和牛奶中乳蛋白含量。然而,Wei等[6]在奶牛饲粮中添加40 g/d过瘤胃赖氨酸,发现乳蛋白含量并无显著提高。Sun等[7]通过体外试验发现,当BMECs中精氨酸(arginine,Arg)浓度为2.80~11.20 mmol/L时,αS1-酪蛋白(CSN1S1)的蛋白表达会随Arg浓度的增加而下调。上述研究表明,奶牛乳腺对于AA的摄取存在着一种适宜的供应模式,高水平的AA供应促进乳蛋白合成的效果并不是最佳的,只有满足适宜的AA供应模式,才能最大限度地促进乳蛋白的合成。

1.2 AA转运调控牛奶乳蛋白合成

AA转运也是影响乳蛋白合成的重要因素之一。Liu等[8]指出,血液中的游离AA可以通过氨基酸转运载体(amino acid transporter,AAT)进入BMECs中合成乳蛋白。Matsumoto等[9]指出,L型氨基酸转运载体1(L type amino acid transporter 1,LAT1)是奶牛乳腺组织摄取AA的主要转运载体之一,当奶牛开始泌乳时,乳腺中LAT1 mRNA表达量会显著升高。Lin等[10]研究发现,增加蛋氨酸(methionine,Met)含量可以显著促进LAT1的蛋白表达,提高Met的转运效率,为乳蛋白合成提供充足的底物。然而,Rulquin等[11]研究发现,给奶牛十二指肠灌注40 g/d亮氨酸(leucine,Leu)可以显著提高乳蛋白合成量,但随着Leu灌注量的增大,AAT在转运AA时会发生竞争性抑制,限制AA的转运,从而降低乳蛋白的合成量。由此可见,AAT在调控乳蛋白合成方面具有重要的调控作用。目前,关于AA转运调控乳蛋白合成方面的研究也较少,每种AA对应的AAT也不同,并且AA在转运时存在相互协同和竞争的关系,需要通过进一步探讨乳腺摄取AA的转运机制以减少AA之间的竞争性抑制,最大限度地提高AA的利用效率,推动平衡AA模式的研究进程。

1.3 AA比例调控牛奶乳蛋白合成

前人研究表明,平衡必需氨基酸比例可以促进乳蛋白合成。吴慧慧[12]在BMECs中添加浓度比例接近15∶5∶9∶10的赖氨酸(lysinine,Lys)、Met、苏氨酸和苯丙氨酸,发现CSN1S1的合成量显著增加。其中,Lys和Met作为乳蛋白合成中的限制性氨基酸,已被证明3∶1的浓度比例是合成乳蛋白的理想比例[13]。Dong等[14]在Lys和Met=3∶1的基础上,使培养基中Lys∶Leu、Lys∶异亮氨酸、Lys∶缬氨酸浓度比例接近0.78∶1、1.29∶1、1.12∶1,发现CSN1S1 mRNA表达量显著上调。综上所述,适宜比例的AA可以上调乳蛋白的基因和蛋白表达,从而促进乳蛋白的合成。目前,AA平衡模式调控乳蛋白的研究大多围绕在Lys、Met之间的平衡比例,需要进一步研究其他AA之间平衡比例,为完善奶牛饲粮配方提供理论参考。

1.4 AA通过mTOR、JAK2-STAT5和GCN2-eIF2α信号通路调控牛奶乳蛋白合成

AA可以激活mTOR信号通路,使下游核糖体S6蛋白激酶1(ribosomal protein S6 kinase 1,S6K1)和翻译起始因子4E结合蛋白1(eukaryotic translation initiation factor 4E-binging protein 1,4EBP1)发生磷酸化,活化后的S6K1通过调控核糖体转录,促进蛋白质的翻译及表达,而磷酸化的4EBP1释放真核翻译启始因子4E(eukaryotic initiation factor 4E,eIF4E),帽结构蛋白eIF4E与RNA解旋酶eIF4A和支架蛋白eIF4G结合形成eIF4F复合体,eIF4F可以打开5'非翻译区的二级结构,促进核糖体与mRNA的5'端的m7G帽结合,从而促进蛋白质的翻译[15]。酪氨酸激酶2-信号转导转录激活因子5(janus kinase 2-signal transducer and activator of transcription 5,JAK2-STAT5)信号通路主要是在基因转录水平调控乳蛋白的合成。Khan等[16]研究发现,AA与细胞膜表面受体相结合,将信号传递给酪氨酸,酪氨酸发生磷酸化并激活JAK2,磷酸化的JAK2促进STAT5形成二聚体,易位到细胞核内,完成膜内外信号的传递,最终与乳蛋白合成相关基因的启动子位点结合,启动基因的转录,促进乳蛋白的合成。周刚[17]给泌乳中期奶牛颈静脉灌注37.66 g/d Arg后,发现产奶量和牛奶中乳蛋白率以及乳腺组织中JAK2、STAT5和CSN1S1 mRNA表达量显著升高。一般性调控阻遏蛋白激酶2-翻译起始因子2(general regulation of blocking protein kinase 2-translation initiation factor 2,GCN2-eIF2α)信号通路能够感知细胞内AA水平的高低,当AA缺失导致tRNA空载时,GCN2与未带电tRNA结合而被激活,引起下游蛋白eIF2α的磷酸化,活化的eIF2α降低mRNA的整体翻译速率,减少AA的消耗[18]。Ruizcortés等[19]研究发现,当细胞内Leu不足时,GCN2下游因子eIF2α会发生磷酸化,磷酸化eIF2α会抑制eIF2α与GTP结合的能力,从而限制了eIF2α-GTP-tRNAiMet三联体的形成,抑制新的翻译起始,减少AA的消耗。这表明GCN2-eIF2α信号通路在维持AA平衡方面发挥重要作用。综上可知,mTOR、JAK2-STAT5和GCN2-eIF2α信号通路同时参与调控乳蛋白的合成,这提示乳腺在乳蛋白合成的调控中可能存在的共同交汇点。因此,AA对乳蛋白合成的调控作用是否存在共同的交汇点尚需进一步研究探索。

2 GLU对牛奶乳蛋白合成的调控作用及其机理

2.1 GLU供应调控牛奶乳蛋白合成

GLU是动物机体中维持生命活动的主要能源物质,可以为乳蛋白的合成提供所需的能量。研究表明,高产奶牛每日需要2 kg GLU才能满足其泌乳需求,占奶牛乳腺摄取GLU总量的60%~85%[20]。Rigout等[21]通过给奶牛十二指肠灌注443和963 g/d GLU,发现增加GLU供应可以通过糖酵解途径为乳蛋白合成提供更多的能量。此外,通过给奶牛饲喂富含淀粉的饲粮,可以使其在消化过程中转化为GLU,增加血液中GLU的供应,提高乳蛋白产量。Rius等[22]研究表明,通过给奶牛皱胃灌注2 kg/d 淀粉,可以显著提高动脉血浆中GLU含量,刺激胰岛素的分泌,促进乳腺内AA的摄取和转运,提高产奶量和牛奶中乳蛋白率。

2.2 GLU转运调控牛奶乳蛋白合成

GLU通过BMECs膜上的葡萄糖转运载体(glucose transporter,GLUT)进入细胞内,因此BMECs膜上GLUT的活性能够影响乳腺对GLU的摄取。Abbas等[23]研究发现,GLUT1、GLUT8和GLUT12可以调控BMECs摄取GLU。母晓佳等[24]研究发现,在BMECs中添加14 mmol/L GLU混合物能显著上调了GLUT1、GLUT8和GLUT12 mRNA表达量,促进BMECs对GLU的摄取,为乳蛋白的合成提供充足的能量。然而,随着GLU供应的增加,乳腺对于GLU的摄取会相对减少。李子南[25]研究发现,当GLU浓度为10.5~21 mmol/L时,BMECs中GLUT1、GLUT8和GLUT12 mRNA表达量会随GLU浓度的升高而下降,GLU的摄取量也会受到限制,降低GLU对BMECs内信号转导通路的调节作用,从而影响BMECs内乳蛋白的合成。

2.3 GLU通过AMPK-mTOR信号通路调控牛奶乳蛋白合成

除了作为乳蛋白合成的能量底物,GLU还可以通过AMPK-mTOR信号通路调控乳蛋白的合成。AMPK作为细胞代谢的能量传感器,能够对机体能量的变化做出快速反应。当机体摄取GLU后,体内AMP/ATP比值降低,抑制AMPK发生磷酸化,上调mTOR复合体1(mTOR complex 1,mTORC1)以及下游关键信号蛋白S6K1的活性,活化后的S6K1通过调控核糖体转录,促进蛋白质的翻译及表达[26]。Sun等[27]在BMECs中添加17.5 mmol/L的GLU后,显著降低了AMPK mRNA表达量,显著上调了mTORS6K1和CSN1S1 mRNA表达量,从而促进乳蛋白的合成。Yu等[28]在BMECs中添加25 mmol/L GLU,发现AMPK的蛋白表达显著低于无GLU组,mTOR、S6K1和β-酪蛋白的蛋白表达显著高于无GLU组,为了进一步验证GLU通过AMPK-mTOR调控乳蛋白的合成,将AMPK基因沉默后,发现mTOR和S6K1的蛋白表达显著上调,更加说明GLU的添加可以抑制AMPK活性,上调mTOR的表达,促进乳蛋白的合成。

3 FA对牛奶乳蛋白合成的调控作用及其机理

3.1 FA供应调控牛奶乳蛋白合成

FA不仅参与乳脂肪的合成,还能一定程度上调节乳蛋白的合成。研究表明,在泌乳前期奶牛饲粮中添加一定比例的脂肪,可以在体内分解产生FA,FA不仅能够缓解奶牛的能量负平衡状态,还可以增加产奶量和改善乳品质[29]。刘瑞芳等[30]给泌乳前期奶牛饲喂脂肪含量为2.54%和6.5%的饲粮,发现6.5%脂肪含量的饲粮可以缓解奶牛的能量负平衡状态,促进乳腺对营养物质摄入,提高牛奶中乳蛋白含量。Santos等[31]研究发现,在奶牛饲粮中添加3%棕榈酸可以为奶牛乳腺提供更多的能量,显著提高产奶量以及乳蛋白含量。Yonezawa等[32]在BMECs中添加400 μmol/L棕榈酸、硬脂酸和亚油酸,发现CSN1S1的蛋白表达显著上调。

3.2 FA转运调控牛奶乳蛋白合成

FA的跨膜过程涉及多个蛋白的协同作用。首先,血液中的游离FA在脂肪酸转运蛋白(fatty acid transport protein,FATP)和分化抗原簇36(cluster of differentiation 36,CD36)的协同作用下进入细胞内,胞质中脂肪酸结合蛋白(fatty acid binding protein,FABP)具有极强的FA亲和力,通过与FA形成共价键的方式,将其运送到线粒体和内质网中进行β-氧化以及脂质合成[33]。李峰[34]研究表明,在BMECs中添加100 μmol/L硬脂酸,FATP3和FATP4 mRNA表达量显著上调,同时β-酪蛋白的蛋白表达也显著上调。这表明FATP在响应外源性FA刺激中发挥关键作用,通过加强FA的跨膜转运,促进BMECs内乳蛋白的合成。

3.3 FA通过AMPK-ACC-CPT1和AMPK-SREBP-1-FASN信号通路调控牛奶乳蛋白合成

FA可以介导AMPK-ACC-CPT1和AMPK-SREBP-1-FASN信号通路调节细胞内FA的合成与氧化过程,从而满足能量需求。当机体能量不足时,AMPK发生磷酸化,抑制下游靶点乙酰辅酶A羧化酶(acetyl-CoA carboxylase,ACC)的活性,然后通过减弱丙二酸单酰辅酶A对肉碱棕榈酰转移酶-1(carnitine palmityl transferase-1,CPT-1)的抑制作用,促进FA进入线粒体内,进而增强了FA的氧化,为乳蛋白的合成提供ATP[35]。此外,活化的AMPK还会抑制固醇调节元件结合蛋白-1(sterol-regulatory element binding protein-1,SREBP-1)以及脂肪酸合成酶(fatty acid synthase,FASN)活性,从而减少FA的合成以及ATP消耗。李红磊等[36]研究发现,在BMECs中添加0.5 μmol/L亚麻酸可以显著上调细胞内SREBP-1、FASNCSN1S1和CSN3 mRNA表达量。

4 AA与GLU互作对牛奶乳蛋白合成的调控作用及其机理

AA和GLU作为动物机体代谢中的重要底物,在乳蛋白合成过程中存在相互协同的效应。GLU供应充足不仅可以提供大量ATP,还能够节省部分生糖氨基酸,增加乳蛋白的合成量。同时,乳腺细胞内部分AA在转氨酶的作用下形成α-酮酸,经过α-酮酸脱氢酶复合体氧化脱羧形成琥珀酰辅酶A,进入三羧酸循环,为乳蛋白的合成提供能量,其余AA则用于合成乳蛋白和其他代谢产物[37]。此外,在AA和GLU缺乏情况下,BMECs中乳蛋白的合成也会受到限制。Zhang等[38]研究发现,将培养基中AA和GLU的浓度从7.20和17.5 mmol/L降低至1.03和2.50 mmol/L后,相比只降低GLU或AA,组合降低组BMECs的相对增殖率和β-酪蛋白的蛋白表达量会显著降低。
AA与GLU协同作用可以增强mTOR信号通路相关蛋白表达并促进乳蛋白合成。AA可以激活Rag蛋白复合体,活化的Rag蛋白复合体与mTOR中调节亚基(regulatory-associated protein of mTOR,Raptor)发生特异性结合,在Ragulator复合体作用下,将mTORC1招募到具有脑Ras同源蛋白(Ras homolog enriched in brain,Rheb)的溶酶体上,从而使Rheb能够结合并激活mTORC1,促进蛋白质的合成[39]。当GLU摄取量增加时,AMPK的活性受到抑制,降低下游结节性硬化复合体(tuberous sclerosis complex,TSC)的活性,促进Rheb与mTORC1结合,活化的mTORC1激活下游蛋白S6K1,促进蛋白质的翻译[40]。王珊珊[41]研究发现,与单独添加组相比,组合添加7.20 mmol/L AA和17.5 mmol/L GLU可以显著提高mTOR和S6K1的磷酸化水平。综上可知,AA与GLU在调控乳蛋白合成的过程中存在互作效应,但是关于单个AA和GLU互作调控乳蛋白合成的研究较少,考虑到体内营养因子复杂交互的原因,应该将体内体外试验相结合,从转录和翻译水平进一步研究单个AA与GLU互作调控牛奶乳蛋白合成的具体机制。

5 AA与FA互作对牛奶乳蛋白合成的调控作用及其机理

AA和FA在影响乳蛋白合成的过程中也存在相互作用。FA供应充足时,通过β氧化分解产生乙酰辅酶A,部分乙酰辅酶A在乙酰乙酰硫解酶作用下形成乙酰乙酰辅酶A,经过羟甲基戊二单酰辅酶A裂解酶作用下转变成酮体,然后进入三羧酸循环,通过氧化过程产生ATP。这样不仅为乳蛋白的合成提供充足的能量,还能够减少部分生酮氨基酸的浪费,保证乳蛋白合成的底物充足。Purdie等[42]研究发现,给奶牛单独灌注400 g/d乙酸盐后,乳蛋白含量无显著变化,但组合灌注400 g/d乙酸盐和300 g/d AA后,牛奶乳蛋白含量显著增加。
AA和FA可以通过调节BMECs中mTOR-SREBP-1信号转导途径来影响乳蛋白的合成。AA不仅可以通过mTORC1激活下游蛋白S6K1和eIF4E,促进蛋白质转录和翻译,还能够通过mTORC1激活SREBP-1,促进FA的合成,FA通过β氧化分解产生乙酰辅酶A,进入三羧酸循环产生ATP,为乳蛋白的合成提供能量[43]。此外,FA的摄入会抑制AMPK以及下游蛋白TSC的活性,促进Rheb与mTORC1结合并发生磷酸化,从而调节乳蛋白的合成[44]。赵艳丽[45]研究发现,在BMECs中添加1.8 mmol/L Leu可以显著上调mTOR和SREBP-1蛋白表达量。Li等[15]用100 μmol/L硬脂酸处理BMECs后,发现mTOR、SREBP-1和β-酪蛋白的蛋白表达显著上调,通过RAPA抑制剂抑制mTOR的活性,发现SREBP-1和β-酪蛋白的蛋白表达显著下降。这些结果表明,AA和FA可以通过刺激mTOR的活性,上调SREBP-1的蛋白表达,从而促进乳蛋白的合成。Appuhamy等[46]试验表明,在BMECs中单独添加5 mmol/L乙酸或者3.5 mmol/L AA,可以上调mTOR蛋白表达,但差异不显著;而当组合添加乙酸与AA时,mTOR的蛋白表达显著上调。综上所述,AA与FA在调控乳蛋白合成的过程中存在互作效应。目前,AA与FA互作影响牛奶乳蛋白合成相关方面的研究较少,只是从转录和翻译水平上探讨了其影响机理,具体的调控作用仍存在争议,这可能是由于在不同试验下,AA和FA的种类、含量以及平衡比例和动物的生理状况的不同所导致。因此,需要大量基础试验研究AA和FA的适宜剂量和比例,并利用基因过表达或沉默、通路阻断等手段验证AA与FA通过信号通路调控牛奶乳蛋白的合成,以更好地解释其调控机理。

6 GLU与FA互作对牛奶乳蛋白合成的调控作用及其机理

GLU和FA在牛奶乳蛋白的合成过程中可能存在互作效应。GLU可以通过糖酵解为FA的代谢提供能量,促进FA的氧化分解产生乙酰辅酶A,进入三羧酸循环,产生更多的ATP,为乳蛋白的合成提供充足的能量[47]。Brossillon等[48]研究发现,相比于在奶牛饲粮中只添加27.1%的玉米颗粒,组合添加3%的亚麻籽油和27.1%的玉米颗粒后,亚麻籽油和玉米颗粒可以通过降解产生α-亚麻酸和GLU,提高饲粮中总FA含量和能量水平,显著提高产奶量,同时乳蛋白含量也有增加的趋势。此外,FA的摄取还可以激活FA合成途径,促进脂肪细胞分化,提高乳腺的外周胰岛素敏感性,从而提高乳腺对于GLU利用效率,促进乳蛋白的合成[49]
GLU和FA可以通过抑制细胞内AMPK的活性,激活下游ACC、SREBP-1、mTORC1及其下游蛋白S6K1和eIF4E,调节FA的合成与氧化以及蛋白质的转录与翻译,从而促进乳蛋白的合成。张花[50]在BMECs中组合添加17.5 mmol/L GLU和14.54 mmol /L FA后,发现mTORS6K1、ACCCSN3 mRNA表达量显著高于GLU组。与上述结果相似,Lin等[51]在BMECs中组合添加17.5 mmol/L GLU和12.0 mmol/L乙酸钠,发现细胞中SREBP-1和FASN mRNA表达量和ACC、FASN和S6K1蛋白表达显著高于GLU组。这说明GLU和FA互作对于乳蛋白合成的调控作用要优于单一添加组。综上所述,GLU和FA互作可以促进牛奶乳蛋白的合成,但是由于目前的相关研究较少,是否存在其他具体机制尚不清楚,还需要进一步的研究探讨。

7 小结

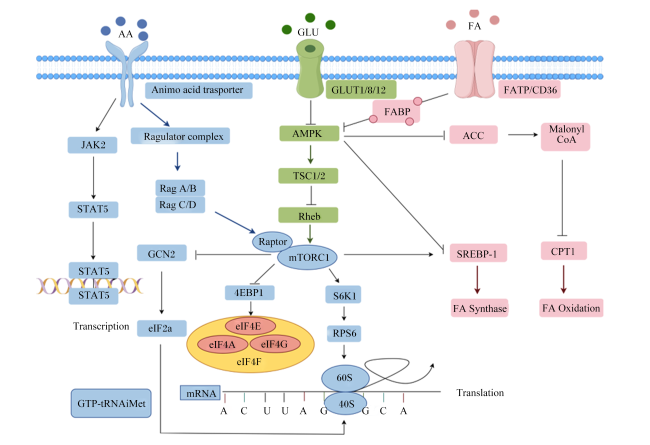
AA、GLU和FA不仅可以直接参与乳蛋白的合成过程中,还可以通过AMPK-mTOR、JAK2-STAT5和GCN2-eIF2a等信号通路调节乳蛋白的合成(图1)。然而,这3种营养性底物对乳蛋白合成的调控作用并不完全一致,可能是由于各底物之间存在着剂量效应以及互作效应,目前关于营养性底物的互作效应对乳蛋白合成的影响机理尚不明确,有待于进一步研究和探讨。值得注意的是,提高某一底物的利用率对于乳蛋白合成的影响终究有限,应该从互作效应方面考虑营养性底物对牛奶乳蛋白合成的影响,为未来科学饲养奶牛提供精准的理论指导。
图1 AA 、GLU和FA互作对AMPK-mTOR、JAK2-STAT5和 GCN2-eIF2a信号通路的调控机制

AA:氨基酸 amino acid;GLU:葡萄糖 glucose;FA:脂肪酸 fatty acid;GLUT1/8/12:葡萄糖转运载体1/8/12 glucose transporter 1/8/12;FATP:肪酸转运蛋白 fatty acid transporter;CD36:分化抗原簇36 differentiation antigen cluster 36;FABP:脂肪酸结合蛋白 fatty acid binding proteins;Ragulator complex:Rag调节蛋白复合体 Rag regulatory protein complex;Rag A/B:Ras相关GTP结合蛋白 A/B Ras-associated GTP binding protein A/B;Rag C/D:Ras相关GTP结合蛋白 C/D Ras-associated GTP binding protein C/D;AMPK:腺苷酸活化蛋白激酶 adenylate activates protein kinase;TSC1/2:结节性硬化复合体1/2 nodular sclerosis complex 1/2;Rheb:脑Ras同源蛋白 brain Ras homologous protein;Raptor:mTOR调节亚基 mTOR regulatory subunit;mTORC1:哺乳动物雷帕霉素靶蛋白复合体 1 mammalian target protein complex of rapamycin 1;4EBP1:翻译起始因子4E结合蛋白1 translation initiation factor 4E-binding protein 1;eIF4E:真核翻译启始因子4E eukaryotic translation initiation factor 4E;eIF4A:真核翻译启始因子4A eukaryotic translation initiation factor 4A;eIF4G:真核翻译启始因子4G eukaryotic translation initiation factor 4G;eIF4F:真核翻译启始因子4F eukaryotic translation initiation factor 4F;S6K1:核糖体S6蛋白激酶1 ribosome S6 protein kinase 1;RPS6:核糖体蛋白S6 ribosomal protein S6;SREBP-1:固醇调节元件结合蛋白-1 sterol regulatory element binding protein-1;ACC:乙酰辅酶A羧化酶 acetyl-coa carboxylase;Malonyl CoA:丙二酸单酰辅酶A malony CoA;CPT-1:肉碱棕榈酰转移酶-1 carnitine palmitoyl transferase-1;JAK2:酪氨酸激酶2;STAT5:信号转导转录激活因子5 signal transduction transcriptional activator 5;GCN2:一般性调控阻遏蛋白激酶2 general regulation of repressor kinase 2;eIF2α:翻译起始因子2 translation initiation factor 2;GTP-tRNAiMet:三磷酸鸟苷-甲硫氨酸-tRNAiMet复合物 guanosine triphosphate-methionine -tRNAiMet complex;60S:60S核糖体蛋白 60S ribosomal protein;40S:40S核糖体蛋白 40S ribosomal protein。

Fig.1 Mechanism of AA,GLU and FA interactions on the regulation of AMPK-mTOR, JAK2-STAT5 and GCN2-eIF2a signaling pathways

[1]
CASTRO J J, HWANG G H, SAITO A, et al. Assessment of the effect of methionine supplementation and inclusion of hydrolyzed wheat protein in milk protein-based milk replacers on the performance of intensively fed Holstein calves[J]. Journal of Dairy Science, 2016, 99(8):6324-6333.

DOI PMID

[2]
ZHANG S H, ZENG X F, REN M, et al. Novel metabolic and physiological functions of branched chain amino acids: a review[J]. Journal of Animal Science and Biotechnology, 2017, 8:10.

DOI PMID

[3]
BAUMGARD L H, WHEELOCK J B, SANDERS S R, et al. Postabsorptive carbohydrate adaptations to heat stress and monensin supplementation in lactating Holstein cows[J]. Journal of Dairy Science, 2011, 94(11):5620-5633.

DOI PMID

[4]
孙振稳. 氨基酸、 葡萄糖和胰岛素对奶牛乳腺上皮细胞增殖及乳蛋白合成的影响[D].硕士学位论文. 泰安: 山东农业大学, 2018.

SUN Z W. Effects of amino acids,glucose and insulin on the proliferation of mammary epithelial cells and milk protein synthesis in dairy cows[D].Master's Thesis. Tai’an: Shandong Agricultural University, 2018. (in Chinese)

[5]
ZHAO K, LIU W, LIN X Y, et al. Effects of rumen-protected methionine and other essential amino acid supplementation on milk and milk component yields in lactating Holstein cows[J]. Journal of Dairy Science, 2019, 102(9):7936-7947.

DOI PMID

[6]
WEI X S, WU H, WANG Z X, et al. Rumen-protected lysine supplementation improved amino acid balance,nitrogen utilization and altered hindgut microbiota of dairy cows[J]. Animal Nutrition, 2023, 15:320-331.

[7]
SUN M, CAO Y, XING Y Y, et al. Effects of L-arginine and arginine-arginine dipeptide on amino acids uptake and αS1-casein synthesis in bovine mammary epithelial cells[J]. Journal of Animal Science, 2023, 101:skad339.

[8]
LIU H Y, WEI X S, DAI W T, et al. The functional and regulatory entities underlying free and peptide-bound amino acid transporters in the bovine mammary gland[J]. JDS Commun, 2023, 4(3):235-239.

[9]
MATSUMOTO T, NAKAMURA E, NAKAMURA H, et al. Production of free glutamate in milk requires the leucine transporter LAT1[J]. American Journal of Physiology.Cell Physiology, 2013, 305(6):C623-C631.

[10]
LIN Y, DUAN X Y, LV H, et al. The effects of L-type amino acid transporter 1 on milk protein synthesis in mammary glands of dairy cows[J]. Journal of Dairy Science, 2018, 101(2):1687-1696.

[11]
RULQUIN H, PISULEWSKI P M. Effects of graded levels of duodenal infusions of leucine on mammary uptake and output in lactating dairy cows[J]. The Journal of Dairy Research, 2006, 73(3):328-339.

[12]
吴慧慧. 必需氨基酸及蛋氨酸二肽供给模式对奶牛乳腺组织αs-酪蛋白合成的影响[D].博士学位论文. 杭州: 浙江大学, 2007.

WU H H. Effect of amine acids pattern and methionylmethinoine on the synthesis of αs-casein in cultured bovine mammary tissue[D].Ph.D.Thesis. Hangzhou: Zhejiang University, 2007. (in Chinese)

[13]
ZHAO Z W, MA Z Y, WANG H, et al. Effects of rumen-protected methionine and lysine supplementation on milk yields and components,rumen fermentation,and the rumen microbiome in lactating yaks (Bos grunniens)[J]. Animal Feed Science and Technology, 2021, 277:114972.

[14]
DONG X, ZHOU Z, WANG L, et al. Increasing the availability of threonine,isoleucine,valine,and leucine relative to lysine while maintaining an ideal ratio of lysine:methionine alters mammary cellular metabolites,mammalian target of rapamycin signaling,and gene transcription[J]. Journal of Dairy Science, 2018, 101(6):5502-5514.

[15]
LI F, HU G Q, LONG X Y, et al. Stearic acid activates the PI3K-mTOR-4EBP1/S6K and mTOR-SREBP-1 signaling axes through FATP4-CDK1 to promote milk synthesis in primary bovine mammary epithelial cells[J]. Journal of Agricultural and Food Chemistry, 2022, 70(13):4007-4018.

[16]
KHAN M Z, KHAN A, XIAO J X, et al. Role of the JAK-STAT pathway in bovine mastitis and milk production[J]. Animals, 2020, 10(11):2107.

[17]
周刚. 精氨酸调控酪蛋白表达途径相关miRNAs的筛选与表达分析[D].硕士学位论文. 扬州: 扬州大学, 2016.

ZHOU G. Screening and expression analysis of miRNAs involved in regulation of casein synthesis by arginine[D].Master's Thesis. Yangzhou: Yangzhou University, 2016. (in Chinese)

[18]
汪东阳, 谢月琴, 罗君谊, 等. 调控乳蛋白合成信号通路的研究进展[J]. 中国奶牛, 2020(5):6-11.

WANG D Y, XIE Y Q, LUO J Y, et al. Research progress in regulating the signal pathway of milk protein synthesis[J]. China Dairy Cattle, 2020(5):6-11. (in Chinese)

[19]
RUIZ-CORTÉS Z T, YODER P, HANIGAN M D. Effects of essential amino acid deficiency on general control nonderepressible 2/eukaryotic initiation factor 2 signaling and proteomic changes in primary bovine mammary epithelial cells[J]. Current Issues in Molecular Biology, 2022, 44(3):1075-1086.

[20]
BICKERSTAFFE R, ANNISON E F, LINZELL J L. The metabolism of glucose acetate,lipids and amino acids in lactating dairy cows[J]. Journal of Agricultural Science, 1974, 82(1):71-85.

[21]
RIGOUT S, LEMOSQUET S, VAN EYS J E, et al. Duodenal glucose increases glucose fluxes and lactose synthesis in grass silage-fed dairy cows[J]. Journal of Dairy Science, 2002, 85(3):595-606.

DOI PMID

[22]
RIUS A G, APPUHAMY J A D R N, CYRIAC J, et al. Regulation of protein synthesis in mammary glands of lactating dairy cows by starch and amino acids[J]. Journal of Dairy Science, 2010, 93(7):3114-3127.

DOI PMID

[23]
ABBAS Z, SAMMAD A, HU L R, et al. Glucose metabolism and dynamics of facilitative glucose transporters (GLUTs) under the influence of heat stress in dairy cattle[J]. Metabolites, 2020, 10(8):312.

[24]
母晓佳, 李大彪, 孙梅, 等. 葡萄糖和泌乳相关激素组合添加对奶牛乳腺上皮细胞酪蛋白合成的影响[J]. 动物营养学报, 2022, 34(9):6072-6087.

DOI

MU X J, LI D B, SUN M, et al. Effects of combination of glucose and lactation related hormones on casein synthesis in bovine mammary epithelial cells[J]. Chinese Journal of Animal Nutrition, 2022, 34(9):6072-6087. (in Chinese)

DOI

[25]
李子南. 葡萄糖对奶牛乳腺上皮细胞能量代谢和酪蛋白合成的影响[D].硕士学位论文. 呼和浩特: 内蒙古农业大学, 2020.

LI Z N. Effect of glucose on energy metabolism and casein synthesis in bovine mammary epithelial cells[D].Master's Thesis. Hohhot: Inner Mongolia Agricultural University, 2020. (in Chinese)

[26]
WANG X L, XU J, ZENG H F, et al. Enhancement of BCAT2-mediated valine catabolism stimulates β-casein synthesis via the AMPK-mTOR signaling axis in bovine mammary epithelial cells[J]. Journal of Agricultural and Food Chemistry, 2022, 70(32):9898-9907.

DOI PMID

[27]
SUN M, LI Z N, XING Y Y, et al. Effects of glucose availability on αS1-casein synthesis in bovine mammary epithelial cells[J]. Journal of Animal Science, 2022, 100(11):skac330.

[28]
YU W, GUO J Q, MAO L, et al. Glucose promotes cell growth and casein synthesis via ATF4/Nrf2-Sestrin2-AMPK-mTORC1 pathway in dairy cow mammary epithelial cells[J]. Animal Biotechnology, 2023, 34(8):3808-3818.

[29]
BELURY M A. Conjugated dienoic linoleate: a polyunsaturated fatty acid with unique chemoprotective properties[J]. Nutrition Reviews, 1995, 53(4 Pt 1):83-89.

PMID

[30]
刘瑞芳, 苏利红. 不同水平亚麻籽对瘤胃内环境及奶牛产奶性能的影响[J]. 饲料工业, 2021, 42(23):5-9.

LIU R F, SU L H. Effects of different levels of flaxseed on rumen environment and milk performance of dairy cows[J]. Feed Industry, 2021, 42(23):5-9. (in Chinese)

[31]
SANTOS N J M, SOUZA J, LOCK A L. Nutrient digestibility and production responses of lactating dairy cows when saturated free fatty acid supplements are included in diets:a Meta-analysis[J]. Journal of Dairy Science, 2021, 104(12):12628-12646.

[32]
YONEZAWA T, YONEKURA S, KOBAYASHI Y, et al. Effects of long-chain fatty acids on cytosolic triacylglycerol accumulation and lipid droplet formation in primary cultured bovine mammary epithelial cells[J]. Journal of Dairy Science, 2004, 87(8):2527-2534.

DOI PMID

[33]
QIN X H, LIU P, JIN L Y, et al. Exerkine β-aminoisobutyric acid protects against atrial structural remodeling and atrial fibrillation in obesity via activating AMPK signaling and improving insulin sensitivity[J]. Biomedicine & Pharmacotherapy, 2024, 171:116137.

[34]
李峰. 硬脂酸对奶牛乳腺上皮细胞中乳脂乳蛋白合成的影响及其机制[D].硕士学位论文. 长春: 吉林大学, 2022.

LI F. Effect and its mechanisms of stearic acid on synthesis of milk fat and milk protein in bovine mammary epithelial cells[D].Master's Thesis. Changchun: Jilin University, 2022. (in Chinese)

[35]
BIONAZ M, LOOR J J. Gene networks driving bovine milk fat synthesis during the lactation cycle[J]. BMC Genomics, 2008, 9:366.

DOI PMID

[36]
李红磊. 二、三维培养模式下添加十八碳不饱和脂肪酸对奶牛乳腺上皮细胞乳成分合成的影响[D].硕士学位论文. 呼和浩特: 内蒙古农业大学, 2016.

LI H L. Effect of 18-carbon unsaturated fatty acids supplementation on milk composition synthesis in two and three-dimensional cultured bovine mammary epithelial cells[D].Master's Thesis. Hohhot: Inner Mongolia Agricultural University, 2016. (in Chinese)

[37]
WEBB L A, SADRI H, SCHUH K, et al. Branched-chain amino acids:abundance of their transporters and metabolizing enzymes in adipose tissue,skeletal muscle,and liver of dairy cows at high or normal body condition[J]. Journal of Dairy Science, 2020, 103(3):2847-2863.

[38]
ZHANG M C, ZHAO S G, WANG S S, et al. D-glucose and amino acid deficiency inhibits casein synthesis through JAK2/STAT5 and AMPK/mTOR signaling pathways in mammary epithelial cells of dairy cows[J]. Journal of Dairy Science, 2018, 101(2):1737-1746.

DOI PMID

[39]
SANCAK Y, PETERSON T R, SHAUL Y D, et al. The rag GTPases bind raptor and mediate amino acid signaling to mTORC1[J]. Science, 2008, 320(5882):1496-1501.

DOI PMID

[40]
SAITO K, ARAKI Y, KONTANI K, et al. Novel role of the small GTPase Rheb:its implication in endocytic pathway independent of the activation of mammalian target of rapamycin[J]. Journal of Biochemistry, 2005, 137(3):423-430.

[41]
王珊珊. 葡萄糖和氨基酸应激对奶牛乳腺上皮细胞β-酪蛋白及信号通路相关蛋白磷酸化表达的影响[D].硕士学位论文. 呼和浩特: 内蒙古农业大学, 2016.

WANG S S. Effects of glucose and amino acids stress on β-casein and signaling pathways related protein phosphorylation expression of bovine mammary epithelial cells[D].Master's Thesis. Hohhot: Inner Mongolia Agricultural University, 2016. (in Chinese)

[42]
PURDIE N G, TROUT D R, POPPI D P, et al. Milk synthetic response of the bovine mammary gland to an increase in the local concentration of amino acids and acetate[J]. Journal of Dairy Science, 2008, 91(1):218-228.

PMID

[43]
ZHANG J, LIU Z Y, NI Y J, et al. Branched-chain amino acids promote occurrence and development of cardiovascular disease dependent on triglyceride metabolism via activation of the mTOR/SREBP-1/betatrophin pathway[J]. Molecular and Cellular Endocrinology, 2024, 584:112164.

[44]
DOSHI H, SPENGLER K, GODBOLE A, et al. AMPK protects endothelial cells against HSV-1 replication via inhibition of mTORC1 and ACC1[J]. Microbiology Spectrum, 2023, 11(5):e0041723.

[45]
赵艳丽. 乙酸与亮氨酸、乙酸与蛋氨酸互作效应对奶牛乳腺上皮细胞内乳成分合成的影响及其机理研究[D].博士学位论文. 呼和浩特: 内蒙古农业大学, 2016.

ZHAO Y L. Effect and mechanism of interaction of acetate and leucine, acetate and methionine on milk components synthesis in the bovine mammary epithelial cells[D].Ph.D.Thesis. Hohhot: Inner Mongolia Agricultural University, 2016. (in Chinese)

[46]
APPUHAMY J A D R N, NAYANANJALIE W A, ENGLAND E M, et al. Effects of AMP-activated protein kinase (AMPK) signaling and essential amino acids on mammalian target of rapamycin (mTOR) signaling and protein synthesis rates in mammary cells[J]. Journal of Dairy Science, 2014, 97(1):419-429.

DOI PMID

[47]
PARK J H, KWON S, PARK Y M. Extracellular vimentin alters energy metabolism and induces adipocyte hypertrophy[J]. Diabetes & Metabolism Journal, 2024, 48(2):215-230.

[48]
BROSSILLON V, REIS S F, MOURA D C, et al. Production,milk and plasma fatty acid profile,and nutrient utilization in Jersey cows fed flaxseed oil and corn grain with different particle size[J]. Journal of Dairy Science, 2018, 101(3):2127-2143.

[49]
FANG X L, SHU G, ZHANG Z Q, et al. Roles of α-linolenic acid on IGF-I secretion and GH/IGF system gene expression in porcine primary hepatocytes[J]. Molecular Biology Reports, 2012, 39(12):10987-10996.

[50]
张花. 添加脂肪酸和激素对奶牛乳腺上皮细胞乳蛋白和乳脂肪合成的影响[D].硕士学位论文. 呼和浩特: 内蒙古农业大学, 2018.

ZHANG H. Effect of fatty acids and hormone supplementation on milk protein and milk fat synthesis in bovine mammary epithelial cells[D].Master's Thesis. Hohhot: Inner Mongolia Agricultural University, 2018. (in Chinese)

[51]
LIN M, JIANG M C, YANG T Y, et al. Acetate-Induced milk fat synthesis is associated with activation of the mTOR signaling pathway in bovine mammary epithelial cells[J]. Animals, 2022, 12(19):2616.

Outlines

/