

1 材料与方法
1.1 试验设计
表1 不同断奶小母猪生长阶段对应的饲粮净能水平Table 1 NE levels of diets at each growth phase for weaned gilts MJ/kg |
| 体重 Body weight | 组别Groups | |||||
|---|---|---|---|---|---|---|
| NE1 | NE2 | NE3 | NE4 | NE5 | NE6 | |
| 6.0~7.5 kg | 10.00 | 10.21 | 10.43 | 10.64 | 10.85 | 11.07 |
| 7.5~11.0 kg | 9.94 | 10.15 | 10.36 | 10.57 | 10.78 | 10.99 |
| 11.0~15.0 kg | 9.60 | 9.81 | 10.02 | 10.23 | 10.44 | 10.65 |
| 15.0~20.0 kg | 9.62 | 9.83 | 10.03 | 10.23 | 10.44 | 10.64 |
| 20.0~25.0 kg | 9.60 | 9.81 | 10.02 | 10.23 | 10.44 | 10.65 |
1.2 试验饲粮
表2 试验饲粮组成及营养水平(风干基础)Table 2 Composition and nutrient levels of experimental diets (air-dry basis) % |
| 项目 Items | 6.0~7.5 kg | 7.5~11.0 kg | 11.0~15.0 kg | 15.0~20.0 kg | 20.0~25.0 kg | ||||||||||||||||||||
|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|
| A | B | A | B | A | B | A | B | A | B | ||||||||||||||||
| 原料Ingredients | |||||||||||||||||||||||||
| 玉米Corn | 20.39 | 5.78 | 22.11 | 21.01 | 44.15 | 41.32 | 45.65 | 45.01 | 45.60 | 46.87 | |||||||||||||||
| 膨化玉米Extruded corn | 20.00 | 20.00 | 15.00 | 15.00 | |||||||||||||||||||||
| 鱼粉Fish meal | 4.00 | 5.00 | 3.00 | 3.00 | 2.00 | 2.00 | 2.00 | 2.00 | 2.00 | 2.00 | |||||||||||||||
| 乳清粉Dried whey | 10.00 | 20.00 | 6.00 | 10.00 | |||||||||||||||||||||
| 乳清浓缩蛋白 Whey protein concentrate | 4.19 | 7.19 | 3.23 | 3.00 | |||||||||||||||||||||
| 膨化大豆 Extruded soybean | 8.00 | 8.00 | 8.00 | 7.00 | |||||||||||||||||||||
| 豆粕Soybean meal | 8.43 | 10.63 | 22.51 | 23.15 | 19.83 | 20.45 | 19.00 | 20.00 | |||||||||||||||||
| 酶解豆粕 Enzymetreated soybean meal | 22.00 | 24.00 | 12.00 | 12.00 | |||||||||||||||||||||
| 大豆皮Soybean hull | 3.75 | 3.90 | 4.40 | 5.00 | 6.00 | ||||||||||||||||||||
| 小麦Wheat | 4.00 | 7.00 | 15.00 | 6.50 | 16.00 | 16.00 | 16.00 | 16.00 | 16.20 | 16.00 | |||||||||||||||
| 次粉Wheat middling | 2.22 | 2.22 | 2.22 | 2.22 | 2.22 | 2.22 | 2.22 | 2.22 | 2.22 | 2.22 | |||||||||||||||
| 麦麸Wheat bran | 3.00 | 3.00 | 4.00 | 5.00 | 5.00 | ||||||||||||||||||||
| 大豆油Soybean oil | 2.82 | 2.62 | 2.52 | 1.97 | 1.83 | ||||||||||||||||||||
| 磷酸氢钙CaHPO4 | 1.22 | 1.00 | 0.95 | 0.90 | 1.30 | 1.35 | 1.05 | 1.05 | 0.80 | 0.85 | |||||||||||||||
| 石粉Limestone | 0.50 | 0.40 | 0.48 | 0.45 | 1.02 | 0.99 | 0.87 | 0.88 | 0.88 | 0.88 | |||||||||||||||
| L-赖氨酸盐酸盐 L-Lys·HCl | 0.17 | 0.06 | 0.22 | 0.22 | 0.37 | 0.38 | 0.36 | 0.37 | 0.35 | 0.36 | |||||||||||||||
| DL-蛋氨酸DL-Met | 0.12 | 0.13 | 0.11 | 0.16 | 0.12 | 0.16 | 0.10 | 0.14 | 0.10 | 0.13 | |||||||||||||||
| L-苏氨酸L-Thr | 0.09 | 0.05 | 0.10 | 0.12 | 0.15 | 0.16 | 0.14 | 0.16 | 0.14 | 0.15 | |||||||||||||||
| L-色氨酸L-Try | 0.01 | 0.02 | 0.02 | 0.01 | |||||||||||||||||||||
| L-缬氨酸L-Val | 0.00 | 0.02 | 0.05 | 0.05 | 0.06 | 0.05 | 0.04 | 0.05 | |||||||||||||||||
| 蔗糖Sucrose | 2.00 | 2.00 | 2.00 | 2.00 | |||||||||||||||||||||
| 食盐NaCl | 0.30 | 0.30 | 0.20 | 0.10 | 0.25 | 0.25 | 0.25 | 0.25 | 0.20 | 0.20 | |||||||||||||||
| 碳酸氢钠NaHCO3 | 0.60 | 0.60 | 0.60 | 0.60 | 0.20 | 0.20 | 0.20 | 0.20 | 0.20 | 0.20 | |||||||||||||||
| 植酸酶Phytase | 0.02 | 0.02 | 0.02 | 0.02 | 0.02 | 0.02 | 0.02 | 0.02 | 0.02 | 0.02 | |||||||||||||||
| 氧化锌ZnO | 0.20 | 0.20 | 0.20 | 0.20 | |||||||||||||||||||||
| 氯化胆碱 Choline chloride | 0.05 | 0.05 | 0.05 | 0.05 | 0.05 | 0.05 | 0.05 | 0.05 | 0.05 | 0.05 | |||||||||||||||
| 二氧化钛TiO2 | 0.40 | 0.40 | 0.40 | 0.40 | 0.40 | 0.40 | 0.40 | 0.40 | 0.40 | 0.40 | |||||||||||||||
| 预混料Premix1) | 0.78 | 0.78 | 0.78 | 0.78 | 0.78 | 0.78 | 0.78 | 0.78 | 0.78 | 0.78 | |||||||||||||||
| 合计Total | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | 100.00 | |||||||||||||||
| 营养水平Nutrient levels2) | |||||||||||||||||||||||||
| 净能NE/(MJ/kg) | 10.00 | 11.06 | 9.94 | 10.98 | 9.60 | 10.64 | 9.62 | 10.64 | 9.60 | 10.64 | |||||||||||||||
| 总能GE/(MJ/kg) | 15.89 | 16.99 | 16.22 | 17.20 | 15.52 | 16.51 | 15.45 | 16.42 | 15.68 | 16.50 | |||||||||||||||
| 干物质DM | 88.15 | 88.17 | 88.23 | 88.06 | 88.22 | 88.25 | 88.19 | 88.13 | 88.21 | 88.09 | |||||||||||||||
| 总磷TP | 0.71 | 0.63 | 0.59 | 0.53 | 0.52 | 0.71 | 0.63 | 0.59 | 0.53 | 0.52 | |||||||||||||||
| 粗蛋白质CP | 18.66 | 20.93 | 17.63 | 18.54 | 14.98 | 16.34 | 14.07 | 16.30 | 14.35 | 15.68 | |||||||||||||||
| 粗脂肪EE | 2.72 | 5.22 | 3.11 | 5.74 | 3.07 | 4.87 | 1.43 | 6.37 | 3.68 | 5.29 | |||||||||||||||
| 中性洗涤纤维NDF | 8.63 | 5.34 | 8.73 | 8.01 | 13.08 | 10.02 | 10.88 | 7.76 | 11.77 | 9.70 | |||||||||||||||
| 酸性洗涤纤维ADF | 4.24 | 2.56 | 4.34 | 3.77 | 6.86 | 5.38 | 5.73 | 3.78 | 6.41 | 4.76 | |||||||||||||||
| 钙Ca | 0.67 | 0.69 | 0.61 | 0.59 | 0.72 | 0.73 | 0.65 | 0.62 | 0.64 | 0.66 | |||||||||||||||
A:饲粮净能水平最低的饲粮;B:饲粮净能水平最高的饲粮。下表同。A: diet with the lowest net energy level; B: diet with the highest net energy level. The same as below. | |
1)预混料为每千克饲粮提供 The premix provided the following per kg of diets: 6.0 to 7.5 kg and 7.5 to 11.0 kg,VA 9 000 IU,VD3 900 IU,VE 150 mg,VB1 1.15 mg,VB2 3.48 mg,VB3 31.4 mg,VB6 5.3 mg,VB12 18 g,生物素 biotin 0.06 mg,D-泛酸 D-pantothenic acid 10.4 mg,叶酸 folic acid 0.31 mg,Zn 95 mg,Fe 105 mg,Cu 5.8 mg,Mn 3.69 mg,I 0.15 mg,Se 0.29 mg;11.0 to 15.0 kg,VA 6 000 IU,VD3 600 IU,VE 150 mg,VB1 1.03 mg,VB2 3.12 mg,VB3 30.2 mg,VB6 4.0 mg,VB12 16 g,生物素 biotin 0.05 mg,D-泛酸 D-pantothenic acid 9.4 mg,叶酸 folic acid 0.30 mg,Zn 85 mg,Fe 101 mg,Cu 5.3 mg,Mn 3.26 mg,I 0.14 mg,Se 0.26 mg;15.0 to 20.0 kg,VA 5 000 IU,VD3 500 IU,VE 60 mg,VB1 0.97 mg,VB2 2.95 mg,VB3 29.7 mg,VB6 3.3 mg,VB12 15 g,生物素 biotin 0.05 mg,D-泛酸 D-pantothenic acid 8.9 mg,叶酸 folic acid 0.3 mg,Zn 81 mg,Fe 99 mg,Cu 5 mg,Mn 3.06 mg,I 0.14 mg,Se 0.25 mg;20.0 to 25.0 kg,VA 5 000 IU,VD3 500 IU,VE 60 mg,VB1 0.96 mg,VB2 2.93 mg,VB3 29.9 mg,VB6 3.2 mg, VB12 15 g,生物素 biotin 0.05 mg,D-泛酸D-pantothenic acid 8.9 mg,叶酸 folic acid 0.3 mg,Zn 81 mg,Fe 100 mg,Cu 5 mg,Mn 3.03 mg,I 0.14 mg,Se 0.25 mg。 2)净能参考NRC(2012)计算得出,其他营养水平为测定值。NE was calculated with reference to NRC (2012), and the other nutrient levels were measured values. |
1.3 生长性能测定
1.4 养分表观消化率测定
1.5 样品采集
1.6 体成分测定
1.7 结肠内容物短链脂肪酸含量测定
1.8 结肠内容物肠道菌群测定
1.9 统计分析
2 结果与分析
2.1 饲粮净能水平对断奶小母猪生长性能的影响
表3 饲粮净能水平对6.0~25.0 kg断奶小母猪生长性能的影响Table 3 Effects of dietary NE level on growth performance of 6.0 to 25.0 kg weaned gilts |
| 项目 Items | 组别Groups | SEM | P值P-value | ||||||||||||||||||
|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|
| NE1 | NE2 | NE3 | NE4 | NE5 | NE6 | 方差分析 ANOVA | 线性 Linear | 二次 Quadratic | |||||||||||||
| 6.0~7.5 kg | |||||||||||||||||||||
| 平均日增重ADG/g | 192.7 | 184.3 | 231.1 | 275.2 | 210.9 | 249.2 | 10.27 | 0.065 | 0.036 | 0.328 | |||||||||||
| 平均日采食量ADFI/g | 269.7 | 269.1 | 292.0 | 338.7 | 254.5 | 304.7 | 9.47 | 0.100 | 0.309 | 0.390 | |||||||||||
| 料重比F/G | 1.61 | 1.45 | 1.25 | 1.23 | 1.35 | 1.27 | 0.068 | 0.656 | 0.171 | 0.327 | |||||||||||
| 腹泻率 Diarrhea incidence/% | 10.84ab | 17.33ab | 6.66b | 6.67b | 11.51ab | 21.82a | 1.693 | 0.035 | 0.205 | 0.024 | |||||||||||
| 7.5~11.0 kg | |||||||||||||||||||||
| 平均日增重ADG/g | 293.1ab | 369.3a | 255.9b | 318.6ab | 307.2ab | 374.4a | 12.01 | 0.026 | 0.172 | 0.134 | |||||||||||
| 平均日采食量ADFI/g | 460.6ab | 500.9a | 420.3b | 480.1ab | 427.3ab | 478.5ab | 8.63 | 0.028 | 0.625 | 0.337 | |||||||||||
| 料重比F/G | 1.59ab | 1.38ab | 1.64a | 1.54ab | 1.39ab | 1.29b | 0.043 | 0.029 | 0.016 | 0.153 | |||||||||||
| 腹泻率 Diarrhea incidence/% | 4.55b | 7.32b | 5.55b | 13.89ab | 10.00b | 25.33a | 1.987 | 0.006 | 0.001 | 0.140 | |||||||||||
| 11.0~15.0 kg | |||||||||||||||||||||
| 平均日增重ADG/g | 369.1ab | 379.0a | 346.1ab | 406.9a | 386.7a | 309.3b | 8.75 | 0.005 | 0.120 | 0.021 | |||||||||||
| 平均日采食量ADFI/g | 638.1 | 626.2 | 558.0 | 618.2 | 636.8 | 536.0 | 15.25 | 0.213 | 0.164 | 0.775 | |||||||||||
| 料重比F/G | 1.73 | 1.65 | 1.62 | 1.52 | 1.65 | 1.74 | 0.034 | 0.429 | 0.918 | 0.060 | |||||||||||
| 腹泻率 Diarrhea incidence/% | 9.45b | 24.55ab | 11.96ab | 20.10ab | 16.07ab | 32.15a | 2.323 | 0.027 | 0.021 | 0.394 | |||||||||||
| 15.0~20.0 kg | |||||||||||||||||||||
| 平均日增重ADG/g | 599.7ab | 497.2c | 618.2a | 527.9bc | 501.2c | 574.7abc | 11.48 | 0.001 | 0.204 | 0.125 | |||||||||||
| 平均日采食量ADFI/g | 1 014.1a | 824.0b | 925.4ab | 902.8b | 887.1b | 876.8b | 14.99 | 0.002 | 0.025 | 0.100 | |||||||||||
| 料重比F/G | 1.70 | 1.68 | 1.50 | 1.71 | 1.77 | 1.53 | 0.033 | 0.082 | 0.562 | 0.838 | |||||||||||
| 腹泻率 Diarrhea incidence/% | 9.38 | 4.29 | 6.94 | 8.34 | 9.76 | 10.83 | 1.471 | 0.829 | 0.432 | 0.486 | |||||||||||
| 20.0~25.0 kg | |||||||||||||||||||||
| 平均日增重ADG/g | 625.4 | 655.2 | 596.0 | 544.7 | 694.8 | 589.8 | 19.24 | 0.258 | 0.768 | 0.709 | |||||||||||
| 平均日采食量ADFI/g | 1 145.3 | 1 074.4 | 1 035.0 | 1 043.1 | 1 093.8 | 1 006.0 | 21.40 | 0.529 | 0.163 | 0.593 | |||||||||||
| 料重比F/G | 1.84 | 1.65 | 1.75 | 1.93 | 1.61 | 1.71 | 0.038 | 0.148 | 0.426 | 0.801 | |||||||||||
| 腹泻率 Diarrhea incidence/% | 10.00 | 7.12 | 10.74 | 8.11 | 10.91 | 12.48 | 1.013 | 0.671 | 0.327 | 0.449 | |||||||||||
| 6.5 to 25.0 kg | |||||||||||||||||||||
| 平均日增重ADG/g | 411.3 | 421.4 | 401.9 | 416.8 | 429.5 | 410.9 | 5.61 | 0.840 | 0.756 | 0.917 | |||||||||||
| 平均日采食量ADFI/g | 700.1 | 667.1 | 641.1 | 680.8 | 678.7 | 637.6 | 7.89 | 0.177 | 0.123 | 0.753 | |||||||||||
| 料重比F/G | 1.71 | 1.59 | 1.60 | 1.63 | 1.59 | 1.55 | 0.021 | 0.163 | 0.038 | 0.591 | |||||||||||
| 腹泻率 Diarrhea incidence/% | 8.69b | 13.38ab | 8.84b | 13.10ab | 12.30b | 22.73a | 1.302 | 0.005 | 0.002 | 0.072 | |||||||||||
同行数据肩标不同小写字母表示差异显著(P<0.05),相同或无字母表示差异不显著(P>0.05),下表同。 | |
In the same row, values with different lowercase letter superscripts mean significant difference (P<0.05), while with the same or no letter superscripts mean no significant difference (P>0.05). The same as below. |
2.2 饲粮净能水平对断奶小母猪养分表观消化率的影响
表4 饲粮净能水平对6.0~25.0 kg断奶小母猪养分表观消化率的影响Table 4 Effects of dietary NE level on nutrient apparent digestibility of 6.0 to 25.0 kg weaned gilts % |
| 项目 Items | 组别Groups | SEM | P值P-value | |||||||
|---|---|---|---|---|---|---|---|---|---|---|
| NE1 | NE2 | NE3 | NE4 | NE5 | NE6 | 方差分析 ANOVA | 线性 Linear | 二次 Quadratic | ||
| 6.0~7.5 kg | ||||||||||
| 干物质DM | 76.61c | 77.79bc | 78.74abc | 78.70abc | 83.46a | 82.57ab | 0.661 | 0.007 | <0.001 | 0.679 |
| 粗蛋白质CP | 69.45 | 70.89 | 71.97 | 72.05 | 77.74 | 74.98 | 0.933 | 0.141 | 0.012 | 0.897 |
| 粗脂肪EE | 75.69 | 78.83 | 80.72 | 83.76 | 81.95 | 80.28 | 1.168 | 0.456 | 0.165 | 0.156 |
| 中性洗涤纤维NDF | 29.39b | 33.04ab | 27.36b | 23.47b | 51.55a | 51.75a | 3.440 | 0.018 | 0.008 | 0.064 |
| 7.5~11.0 kg | ||||||||||
| 干物质DM | 80.69ab | 79.61b | 79.86b | 81.09ab | 82.30ab | 83.13a | 0.391 | 0.049 | 0.006 | 0.097 |
| 粗蛋白质CP | 73.53 | 72.35 | 70.34 | 70.90 | 74.84 | 73.81 | 0.672 | 0.355 | 0.497 | 0.113 |
| 粗脂肪EE | 74.07a | 77.60a | 63.72b | 76.81a | 79.72a | 81.48a | 1.301 | <0.001 | 0.002 | 0.004 |
| 中性洗涤纤维NDF | 38.69 | 33.16 | 47.28 | 42.92 | 46.68 | 46.57 | 1.858 | 0.169 | 0.046 | 0.720 |
| 11.0 to 15.0 kg | ||||||||||
| 干物质DM | 63.36b | 77.07a | 75.23a | 73.19a | 75.24a | 81.15a | 1.253 | <0.001 | <0.001 | 0.188 |
| 粗蛋白质CP | 52.58b | 71.24a | 68.41a | 64.23a | 69.88a | 73.56a | 1.602 | <0.001 | <0.001 | 0.079 |
| 粗脂肪EE | 39.00b | 62.93a | 60.89a | 49.07ab | 60.54a | 65.88a | 2.494 | 0.007 | 0.009 | 0.398 |
| 中性洗涤纤维NDF | 30.41b | 47.75ab | 42.89ab | 51.75ab | 38.45ab | 58.69a | 2.671 | 0.017 | 0.012 | 0.705 |
| 15.0 to 20.0 kg | ||||||||||
| 干物质DM | 78.56 | 79.93 | 77.80 | 80.54 | 80.90 | 79.56 | 0.424 | 0.308 | 0.215 | 0.704 |
| 粗蛋白质CP | 72.33 | 75.77 | 72.83 | 75.88 | 75.72 | 74.11 | 0.692 | 0.526 | 0.412 | 0.380 |
| 粗脂肪EE | 51.08c | 66.78b | 69.08b | 75.64ab | 81.02a | 81.87a | 2.150 | <0.001 | <0.001 | 0.003 |
| 中性洗涤纤维NDF | 26.51 | 29.24 | 17.60 | 26.92 | 32.95 | 31.29 | 2.188 | 0.484 | 0.329 | 0.331 |
| 20.0 to 25.0 kg | ||||||||||
| 干物质DM | 78.79c | 81.03abc | 80.15bc | 83.38a | 82.76ab | 82.51ab | 0.400 | 0.001 | <0.001 | 0.091 |
| 粗蛋白质CP | 74.63b | 77.22ab | 77.04ab | 80.10a | 78.73ab | 78.57ab | 0.512 | 0.025 | 0.005 | 0.073 |
| 粗脂肪EE | 77.60 | 80.49 | 79.65 | 80.23 | 82.06 | 79.54 | 0.448 | 0.094 | 0.083 | 0.092 |
| 中性洗涤纤维NDF | 26.43b | 38.61ab | 36.61ab | 46.28a | 48.44a | 48.32a | 1.913 | <0.001 | <0.001 | 0.136 |
2.3 饲粮净能水平对25.0 kg断奶小母猪体成分含量的影响
表5 饲粮净能水平对25.0 kg断奶小母猪体成分沉积的影响Table 5 Effects of dietary NE level on body composition deposition of 25.0 kg weaned gilts |
| 项目 Items | 组别Groups | SEM | P值P-value | ||||||||||||||||||||
|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|---|
| ISG | NE1 | NE2 | NE3 | NE4 | NE5 | NE6 | 方差分析 ANOVA | 线性 Linear | 二次 Quadratic | ||||||||||||||
| 体水分 Body moisture/(g/kg) | 691.89 | 696.04 | 703.01 | 706.83 | 707.50 | 709.81 | 695.03 | 2.003 | 0.140 | 0.682 | 0.012 | ||||||||||||
| 体粗蛋白质 Body CP/(g/kg) | 146.35 | 157.52 | 156.83 | 156.29 | 156.16 | 154.47 | 157.02 | 1.468 | 0.990 | 0.771 | 0.744 | ||||||||||||
| 体粗脂肪 Body EE/(g/kg) | 120.34 | 110.31 | 101.98 | 101.23 | 102.55 | 95.26 | 112.26 | 1.791 | 0.050 | 0.781 | 0.009 | ||||||||||||
| 体粗灰分 Body Ash/(g/kg) | 28.60 | 25.99 | 25.95 | 25.31 | 26.31 | 27.18 | 26.67 | 0.438 | 0.891 | 0.401 | 0.722 | ||||||||||||
| 体钙 Body Ca/(g/kg) | 6.97 | 6.84 | 5.94 | 6.22 | 6.60 | 6.65 | 6.76 | 0.183 | 0.694 | 0.581 | 0.323 | ||||||||||||
| 体磷 Body P/(g/kg) | 4.95 | 4.88 | 4.52 | 4.77 | 4.68 | 4.83 | 4.94 | 0.009 | 0.871 | 0.592 | 0.411 | ||||||||||||
| 体水分/体粗蛋白质 Body moisture/body CP | 4.74 | 4.46 | 4.49 | 4.53 | 4.54 | 4.59 | 4.45 | 0.051 | 0.953 | 0.782 | 0.451 | ||||||||||||
| 体粗脂肪/ 体粗蛋白质 Body EE/body CP | 0.82 | 0.71 | 0.65 | 0.65 | 0.66 | 0.62 | 0.72 | 0.011 | 0.273 | 0.931 | 0.044 | ||||||||||||
| 体粗灰分/ 体粗蛋白质 Body Ash/body CP | 0.20 | 0.17 | 0.16 | 0.16 | 0.17 | 0.17 | 0.17 | 0.000 | 0.821 | 0.264 | 0.591 | ||||||||||||
| 体粗蛋白质能量 Energy of body CP/(MJ/kg) | 3.47 | 3.73 | 3.72 | 3.70 | 3.70 | 3.66 | 3.72 | 0.030 | 0.990 | 0.772 | 0.730 | ||||||||||||
| 体粗脂肪能量 Energy of body EE/(MJ/kg) | 4.77 | 4.37 | 4.04 | 4.01 | 4.06 | 3.77 | 4.45 | 0.073 | 0.052 | 0.781 | 0.009 | ||||||||||||
| 体总能 Body GE/(MJ/kg) | 7.80 | 7.66 | 7.42 | 7.27 | 7.31 | 7.13 | 7.47 | 0.081 | 0.611 | 0.332 | 0.170 | ||||||||||||
ISG:初始屠宰组 initial slaughter group。 |
2.4 饲粮净能水平对25.0 kg断奶小母猪体成分沉积速率的影响
表6 饲粮净能水平对25.0 kg断奶小母猪体成分沉积速率的影响Table 6 Effects of dietary NE level on body composition deposition rate of 25.0 kg weaned gilts |
| 项目 Items | 组别Groups | SEM | P值P-value | |||||||
|---|---|---|---|---|---|---|---|---|---|---|
| NE1 | NE2 | NE3 | NE4 | NE5 | NE6 | 方差分析 ANOVA | 线性 Linear | 二次 Quadratic | ||
| 体水分 Body moisture/(g/d) | 259.61 | 278.81 | 258.25 | 285.46 | 281.28 | 270.19 | 4.092 | 0.258 | 0.291 | 0.343 |
| 体粗蛋白质 Body CP/(g/d) | 60.03 | 63.24 | 58.00 | 62.85 | 61.71 | 62.44 | 1.243 | 0.853 | 0.653 | 0.893 |
| 体粗脂肪 Body EE/(g/d) | 40.05 | 37.95 | 34.51 | 37.92 | 34.56 | 42.65 | 1.171 | 0.304 | 0.792 | 0.056 |
| 体粗灰分 Body Ash/(g/d) | 9.37 | 9.89 | 8.82 | 10.00 | 10.52 | 10.10 | 0.249 | 0.473 | 0.206 | 0.807 |
| 体钙 Body Ca/(g/d) | 2.52 | 2.21 | 2.18 | 2.55 | 2.58 | 2.60 | 0.100 | 0.695 | 0.367 | 0.411 |
| 体磷 Body P/(g/d) | 1.80 | 1.73 | 1.72 | 1.81 | 1.88 | 1.92 | 0.054 | 0.894 | 0.336 | 0.512 |
| 体氮 Body N/(g/d) | 9.61 | 10.12 | 9.28 | 10.05 | 9.87 | 9.99 | 0.201 | 0.854 | 0.655 | 0.892 |
| 体总能 Body GE/(MJ/d) | 2.83 | 2.89 | 2.58 | 2.81 | 2.73 | 2.87 | 0.061 | 0.760 | 0.954 | 0.377 |
2.5 饲粮净能水平对断奶小母猪结肠菌群和短链脂肪酸含量的影响
表7 饲粮净能水平对断奶小母猪结肠菌群的影响Table 7 Effects of dietary NE level on colonic microbiota of weaned gilts % |
| 项目 Items | 组别Groups | SEM | P值P-value | |||||||
|---|---|---|---|---|---|---|---|---|---|---|
| NE1 | NE2 | NE3 | NE4 | NE5 | NE6 | 方差分析 ANOVA | 线性 Linear | 二次 Quadratic | ||
| 门水平Phylum level | ||||||||||
| 厚壁菌门Firmicutes | 62.08 | 59.76 | 60.61 | 64.73 | 64.65 | 65.60 | 1.763 | 0.921 | 0.352 | 0.771 |
| 拟杆菌门Bacteroidota | 28.76 | 34.08 | 28.34 | 26.89 | 29.72 | 26.06 | 1.697 | 0.843 | 0.451 | 0.791 |
| 螺旋体门Spirochaetota | 2.23 | 2.02 | 4.92 | 2.87 | 1.01 | 1.22 | 0.414 | 0.052 | 0.180 | 0.051 |
| 变形菌门Proteobacteria | 2.14 | 1.49 | 0.68 | 0.89 | 1.65 | 3.34 | 0.478 | 0.681 | 0.511 | 0.122 |
| 属水平Genus level | ||||||||||
| 毛螺菌科未定级菌 Muribaculaceae_norank | 8.88 | 11.19 | 10.32 | 10.47 | 15.97 | 11.44 | 0.924 | 0.353 | 0.164 | 0.671 |
| 普雷沃氏菌属_9 Prevotella_9 | 2.82 | 6.51 | 4.38 | 4.25 | 3.48 | 6.00 | 0.818 | 0.801 | 0.712 | 0.982 |
| 密螺旋体属 Treponema | 2.25 | 1.98 | 4.95 | 2.86 | 1.04 | 1.21 | 0.230 | 0.051 | 0.192 | 0.053 |
| 未分类的产粪甾醇 真细菌群 [Eubacterium] coprostanoligenes group_ norank | 1.59 | 1.70 | 2.00 | 2.32 | 2.79 | 1.88 | 0.511 | 0.542 | 0.231 | 0.332 |
| 粪杆菌属 Faecalibacterium | 2.53 | 2.84 | 2.26 | 2.77 | 2.11 | 2.50 | 0.200 | 0.911 | 0.682 | 0.991 |
| 八叠球菌属Sarcina | 0.09 | 0.41 | 0.06 | 0.15 | 1.11 | 0.56 | 0.167 | 0.501 | 0.211 | 0.832 |
| 考拉杆菌属 Phascolarctobacterium | 1.16 | 1.74 | 1.06 | 1.75 | 2.05 | 0.82 | 0.341 | 0.312 | 0.991 | 0.221 |
| 罕见小球菌属 Subdoligranulum | 1.05 | 1.33 | 1.02 | 1.78 | 1.34 | 1.95 | 0.143 | 0.352 | 0.082 | 0.733 |
| 瘤胃菌科UCG-005 Ruminaceae UCG-005 | 1.65 | 1.46 | 2.20 | 1.26 | 1.78 | 1.62 | 0.149 | 0.642 | 0.972 | 0.852 |
| 罗氏菌属Roseburia | 3.13 | 1.82 | 1.95 | 1.79 | 1.95 | 1.14 | 0.202 | 0.122 | 0.021 | 0.542 |
| 普氏菌科NK3B31群 Prevotellaceae NK3B31 group | 2.22 | 3.99 | 2.52 | 2.30 | 1.52 | 1.83 | 0.393 | 0.573 | 0.251 | 0.612 |
| 瘤胃球菌属 Ruminococcus | 0.43 | 0.88 | 0.25 | 0.42 | 0.35 | 0.33 | 0.081 | 0.252 | 0.231 | 0.931 |
表8 饲粮净能水平对断奶小母猪结肠内容物中短链脂肪酸含量的影响Table 8 Effects of dietary NE level on short-chain fatty acid contents in colon content of weaned gilts μg/g |
| 项目 Items | 组别Groups | SEM | P值P-value | |||||||
|---|---|---|---|---|---|---|---|---|---|---|
| NE1 | NE2 | NE3 | NE4 | NE5 | NE6 | 方差分析 ANOVA | 线性 Linear | 二次 Quadratic | ||
| 乙酸Acetate | 2 490.3 | 2 197.2 | 2 181.6 | 2 288.6 | 2 198.3 | 2 201.3 | 182.09 | 0.851 | 0.412 | 0.510 |
| 丙酸Propionate | 1 488.2 | 1 145.5 | 1 213.4 | 1 249.7 | 1 107.2 | 1 237.7 | 57.41 | 0.510 | 0.271 | 0.252 |
| 丁酸Butyrate | 939.44 | 637.30 | 700.00 | 689.60 | 692.30 | 883.80 | 47.161 | 0.363 | 0.901 | 0.042 |
| 异丁酸Isobutyrate | 119.26bc | 94.53c | 133.04abc | 141.15abc | 194.50a | 183.03ab | 10.598 | 0.042 | <0.001 | 0.553 |
| 戊酸Valerate | 212.05 | 164.22 | 208.32 | 216.58 | 272.60 | 311.65 | 15.681 | 0.081 | 0.013 | 0.142 |
| 异戊酸Isovalerate | 105.77b | 87.95b | 123.93b | 132.29ab | 190.60a | 191.64a | 11.154 | 0.011 | <0.001 | 0.383 |
2.6 结肠菌群及其代谢产物与腹泻率和料重比之间的相关性分析
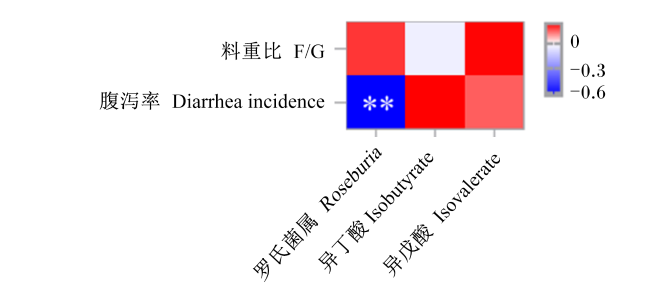


图1 断奶小母猪腹泻率和料重比与结肠菌群和代谢产物的相关性红色表示正相关,蓝色表示负相关,白色表示无相关性。**代表极显著相关(P=0.008)。 Fig.1 Correlation between diarrhea incidence and F/G and microbiota and its metabolites in colon of weaned gilts Red indicated a positive correlation, blue indicated a negative correlation, and white indicated no correlation. ** indicated an extremely significant correlation (P=0.008). |