REVIEW

Biological Functions of Sesamol and Its Application in Livestock and Poultry Production

  • CHEN Sikui , 1 ,
  • HUANG Xingguo 1 ,
  • WANG Xinxia , 2, 3, 4, *
Expand
  • 1 College of Animal Science and Technology, Hunan Agricultural University, Changsha 410128, China
  • 2 College of Animal Science, Zhejiang University, Hangzhou 310058, China
  • 3 Key Laboratory of Molecular Animal Nutrition (Zhejiang University), Ministry of Education, Hangzhou 310058, China
  • 4 Key Laboratory of Animal Nutrition and Feed Science (Eastern of China), Ministry of Agriculture and Rural Affairs, Hangzhou 310058, China
*professor, E-mail:

Received date: 2024-12-26

  Online published: 2025-08-14

Abstract

Sesamol (SEM) is a phenolic compound present in sesame, which has the effects of anti-oxidation, anti-inflammation, anti-obesity, bacteriostasis, anti-tumor, and protection of intestinal barrier, etc. As a natural plant extract, SEM holds great potential for application in livestock and poultry production. This review summarizes the physicochemical properties, main physiological functions and application of SEM in livestock and poultry production, providing a reference for the rational application of SEM in livestock and poultry production.

Cite this article

CHEN Sikui , HUANG Xingguo , WANG Xinxia . Biological Functions of Sesamol and Its Application in Livestock and Poultry Production[J]. Chinese Journal of Animal Nutrition, 2025 , 37(8) : 4966 -4975 . DOI: 10.12418/CJAN2025.406

抗生素用于畜牧业领域已有70余年,在起到促进生长、治疗和预防疾病等作用的同时,也带来了病原菌耐药性的问题[1]。自2020年起,我国规定禁止在饲料中添加抗生素[2],这一转变促进了包括植物提取物在内的多种添加剂在动物饲养中的应用,为畜牧业的可持续发展提供了新的方向。植物多酚是一类天然的植物提取物,具有多种生物学活性。其中,芝麻酚(sesamol,SEM)是从芝麻中提取的一种天然酚类物质,具有抗氧化[3]、抗炎[4]、抗肥胖[5]、抗菌[6]、抗肿瘤[7]以及保护肠道屏障[8]等作用,在畜禽生产上具有良好的应用前景,但目前SEM在畜禽生产上的研究相对较少。因此,本文就SEM的理化性质、生物学功能及其在畜禽生产中的应用等进行综述,为SEM在畜禽生产中的合理应用提供参考。

1 SEM的理化性质
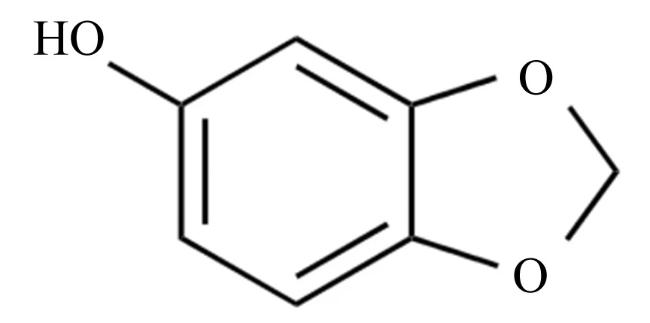
SEM又名3,4-亚甲二氧基苯酚,是一种天然脂溶性木脂素化合物,存在于芝麻籽、芝麻油和芝麻粕中,在芝麻油中的最大值可达644 mg/kg[9]。SEM是一种结晶针状化合物,呈淡棕色并具有奇特的气味,熔点为(64±1) ℃,37 ℃下在水中溶解度为(38.8±1.2) mg/mL[10]。SEM的分子式为C7H6O3,摩尔质量为138.12 g/mol,具有亲脂性和亲水性[11]。SEM的酚类性质使其能够形成酚类自由基来中断自由基链式反应,这些自由基要么二聚化,要么重新排列,形成中性且无毒的成分,从而起到抗氧化作用,保护了机体内其他物质被氧化[12]。SEM化学结构如图1所示。
图1 SEM化学结构

Fig.1 Chemical structure of SEM

2 SEM的生理功能

2.1 抗氧化作用

动物机体在新陈代谢过程中,会产生各种活性氧(reactive oxygen species,ROS),正常生理状态下,由于机体具有抗氧化系统,这些氧化代谢的副产物不会对机体构成威胁。然而,当ROS或自由基产生过量,会打破氧化系统与抗氧化系统间的平衡,过量的自由基会攻击脂质、蛋白质和DNA等生物分子,从而诱发各种疾病[13]。SEM有很强的抗氧化和清除自由基的功能,可以有效清除羟基自由基[14]。有研究表明,SEM能通过电荷转移修复色氨酸自由基,显示出对蛋白质氧化损伤的保护作用,同时还可以有效清除羟基、单电子氧化、有机盐过氧基、脂质过氧基等[15]。还有研究显示,SEM不仅能抑制单链DNA的断裂[16],还能够有效抑制脂质的过氧化反应[17],这有助于保护血浆、低密度脂蛋白和红细胞膜免受氧化。超氧化物歧化酶(superoxide dismutase,SOD)能在歧化反应中清除自由基并产生过氧化氢(H2O2)和氧气(O2)[18],过氧化氢酶(catalase,CAT)主要负责将H2O2分解为氧化氢(H2O)和 O 2 [19],谷胱甘肽过氧化物酶(glutathione peroxidase,GPx)则通过谷胱甘肽(glutathione,GSH)发挥作用[18],它们共同组成动物体内的酶促抗氧化系统[20]。体外试验显示,由外源性H2O2诱导的人神经母细胞瘤细胞经1 μmol/L的SEM预处理3 h能够显著减少细胞死亡以及细胞内ROS的产生,并提高细胞中SOD2和CAT的蛋白表达水平[21]。体内试验表明,经50 mg/kg BW剂量的SEM灌胃处理后,高盐饮食诱导的高血压大鼠红细胞、肝脏、肾脏和心脏中SOD、CAT和GPx活性显著提高,同时还提高了大鼠血浆和组织中的维生素C、维生素E和GSH等非酶抗氧化剂的含量[22]。GSH是一种能够清除自由基的物质,而丙二醛(malondialdehyde,MDA)是脂质过氧化的产物之一[23]。大鼠嗜铬细胞瘤细胞在不同浓度SEM的处理下以剂量依赖的方式显著降低了细胞的MDA含量,并提高了GSH含量[24]。也有研究发现,在卵清蛋白诱导的哮喘小鼠模型中,30 mg/kg BW剂量的SEM提高了肺脏组织中的GSH含量,并降低了MDA含量[25]。NAD(P)H醌氧化还原酶1[NAD(P)H:quinone oxidoreductase 1,NQO1)和血红素加氧酶-1(heme oxygenase-1,HO-1)是核因子红系2相关因子2(nuclear factor erythroid 2-related factor 2,Nrf2)的靶基因,而Nrf2是抵抗氧化应激的关键转录因子[26]。有研究显示,SEM能显著提高Nrf2蛋白水平并上调HO-1和NQO1的mRNA水平[27]。在D-半乳糖诱导的小鼠肝脏氧化应激模型中,SEM能够增加细胞核内的Nrf2含量,促进Nrf2的核转移,进而可能通过调控下游抗氧化酶HO-1、NQO1的表达[28]。综上所述,SEM作为一种天然抗氧化剂,一方面通过自身结构特性清除动物体内的自由基,另一方面可以增强抗氧化酶活性并调节Nrf2信号通路来促进抗氧化基因表达。

2.2 抗炎作用

外界的刺激会激活动物的免疫系统,影响动物的生长和健康状态,从而造成免疫应激,同时机体也会产生炎性反应来缓解免疫应激,炎性反应是动物体处于免疫应激状态的标志。研究表明,在体内环氧合酶(cyclooxygenase,COX)可以催化花生四烯酸形成炎性介质引起炎症反应[29];在葡聚糖硫酸钠诱导的结肠炎小鼠模型中,SEM显著抑制了COX-2的表达[30];一氧化氮(NO)是炎症反应的信号分子[31],而肿瘤坏死因子-α(tumor necrosis factor-α,TNF-α)是激活核转录因子-κB(nuclear factor-κB,NF-κB)的重要炎性介质[32]。在脂多糖诱导的小鼠单核巨噬细胞体外炎症模型中发现,0.5 mg/mL的SEM对NO和TNF-α的生成具有抑制作用[33]。NF-κB信号通路的激活程度可以通过检测磷酸化p65(p-p65)水平来反映,同时NF-κB还有调控白细胞介素-6(interleukin-6,IL-6)、白细胞介素-1β(interleukin-1β,IL-1β)等的作用,IL-6对炎症反应具有调节作用,白细胞介素-1(interleukin-1,IL-1)则是一种强效促炎细胞因子[34]。在小鼠背部涂抹62.5 mg 5%的咪喹莫特乳膏建立的银屑病模型中,在皮肤损伤处涂抹不同浓度的SEM显著降低了TNF-αIL-1βIL-6等炎症因子的基因表达水平,并下调了机体炎症状态[35]。体外试验也表明,不同浓度的SEM能够显著降低脂多糖诱导小鼠单核巨噬细胞中IL-6、IL-1α和IL-1β含量,且呈剂量依赖性[36]。单磷酸腺苷活化蛋白激酶(adenosine monophosphate-activated protein kinase,AMPK)是细胞能量平衡的关键调节器,它参与调控炎症反应,并通过多种途径维持细胞稳态[37]。有研究显示,每日灌胃100 mg/kg BW剂量的SEM可显著降低肥胖小鼠血清和脂肪组织中巨噬细胞分泌的炎症因子IL-6和TNF-α的分泌水平,并显著提高抗炎因子白细胞介素-10(interleukin-10,IL-10)的分泌水平;在其体外研究中,SEM能够激活巨噬细胞的AMPK,同时上调AMPK的下游蛋白过氧化物酶体增殖物激活受体γ辅激活子-1α(peroxisome proliferator-activated receptor gamma coactivator-1α,PGC-1α)以及下调NF-κB的表达[38]。沉默信息调节因子1(silent information regulator transcript 1,SIRT1)是沉默信息调节因子(silent information regulator transcript,SIRT)家族成员之一,具有抗炎和抗氧化应激的作用,与AMPK共同发挥作用[39]。Feng等[40]报道,SEM通过调节AMPK/SIRT1/NF-κB信号通路来改善脊髓损伤小鼠的神经炎症,其具体机制是SEM通过增加SIRT1蛋白的表达和磷酸化AMPK/AMPK比率来上调AMPK/SIRT1通路,同时降低p-p65/p65比率来抑制NF-κB的激活,进一步减少IL-6和TNF-α的释放。综上所述,SEM一方面通过抑制产生炎性介质的酶类活性,减少炎性介质的产生,从而发挥抗炎作用;另一方面通过抑制TNF-α等炎性因子,调节AMPK、SIRT1、NF-κB等信号通路,进而减少炎性因子的表达,起到抑制炎症反应的作用。

2.3 抗肥胖作用

在畜禽生产中,畜禽的脂肪沉积与畜产品品质密切相关。因此,调控畜禽脂肪沉积对于畜禽生产而言至关重要。研究显示,SEM能够显著降低高脂饮食诱导的肥胖小鼠体重增加,并抑制脂肪组织和肝脏中的脂质积累[41],以及降低血浆总胆固醇和甘油三酯含量[42]。过氧化物酶体增殖物激活受体(peroxisome proliferator-activated receptor,PPAR)γ和PPARα是调节脂肪积累的关键转录因子[43],脂肪酸合成酶(fatty acid synthase,FAS)与乙酰辅酶A羧化酶(acetyl-CoA carboxylase,ACC)共同参与脂肪酸合成,而硬脂酰辅酶A去饱和酶1(stearoyl-CoA desaturase 1,SCD1)负责将饱和脂肪酸转化为单不饱和脂肪酸,它们都是调控脂肪沉积的重要因子[44-46]。体外试验表明,3 μg/mL的SEM显著降低了人肝癌细胞内的甘油三酯和总胆固醇含量以及与脂肪合成相关基因(包括FASACCSCD1等)的表达,同时还提高了与脂肪酸氧化相关基因,尤其是PPARα和肉毒碱棕榈酰转移酶(carnitine palmitoyltransferase,CPT)1α表达[47]。Shi等[48]研究也发现,3 μg/mL的SEM处理能激活PPAR信号通路,上调PPARαCPT1α等脂肪酸氧化基因和胆固醇外排及分解相关基因PPARγ的表达,从而加速脂质消耗,减少细胞内的脂质积累。体内试验表明,0.05%(w/v)的SEM抑制了高脂高果糖诱导的肥胖小鼠脂肪生成相关基因PPARγFASACC的表达,同时提高了脂肪分解和线粒体活性相关基因PPARαCPT1αCPT2的表达,并显著抑制了3T3-L1前脂肪细胞的分化和脂滴积累[49]。Hu等[50]报道,100 mg/kg BW剂量的SEM降低了高脂饮食诱导的中年小鼠体重,并减轻了与肥胖相关的代谢综合征,其具体机制是SEM通过激活AMPK,降低了丙酮酸脱氢酶激酶同工酶4(pyruvate dehydrogenase kinase 4,PDK4)和固醇调节元件结合蛋白-1c(sterol regulatory element-binding protein-1c,SREBP-1c)的表达,同时提高葡萄糖转运蛋白4(glucose transporter type 4,GLUT4)的表达,并上调激素敏感性脂肪酶(hormone-sensitive lipase,HSL)的磷酸化和CPT1α水平。其中,HSL主要调节脂肪分解,为能量代谢提供脂肪酸[51];PDK4通过调节糖酵解和氧化代谢的平衡,影响能量的产生和利用[52];SREBP-1c则通过调控脂肪酸和胆固醇的合成,维持脂代谢的平衡[53];GLUT4负责调节葡萄糖的摄取和利用,维持血糖稳定[54]。白色脂肪组织(white adipose tissue,WAT)具有储存能量的作用,而棕色脂肪组织(brown adipose tissue,BAT)是一种具有产热功能的脂肪组织,在能量代谢中起着重要作用,被认为是治疗肥胖的潜在靶点[55]。有研究报道,灌胃100 mg/kg BW剂量的SEM降低了高脂饮食诱导的肥胖小鼠的体脂含量,进一步研究发现,SEM能显著上调脂肪组织中解偶联蛋白1(uncoupling protein 1,UCP1)的水平,并通过上调β3-肾上腺素能受体(β3-adrenergic receptor,β3-AR)和蛋白激酶A(protein kinase A,PKA)信号通路,促进WAT细胞褐变[56]。褐变是WAT在特定条件下转化为BAT的过程,UCP1是脂肪组织褐变的关键标志蛋白[57],β3-AR及PKA则可以驱动WAT中的褐变效应[58-59]。类似的研究发现,SEM能够激活Nrf2,同时提高WAT中UCP1的表达来刺激能量消耗[60]。综上所述,SEM通过调节PPAR、SIRT1/AMPK和β3-AR/PKA等途径来调节与脂质代谢相关的多种蛋白的表达,以此来增加脂肪的分解和脂肪酸氧化以及胆固醇外排及分解,从而改善机体的肥胖症状。

2.4 抗菌作用

有研究表明,SEM对5种食源性病原体(包括单核细胞增生李斯特菌、金黄色葡萄球菌、蜡样芽孢杆菌、大肠杆菌和沙门氏菌)显示出显著的抑制作用,在48 h内的抑制效果在2.16~4.16 lg(CFU/g)[61]。Wu等[6]报道,SEM与乳酸链球菌素组合能够抑制单核细胞增生李斯特菌的生长,并干扰其细胞膜的功能和形态。Yenn等[62]研究发现,芝麻油提取物对8种测试微生物中的4种革兰氏阳性细菌和2种革兰氏阴性细菌表现出敏感性,显示出广谱抗菌活性,该提取物最小抑制浓度为3.1~12.5 mg/mL,最小杀菌浓度为6.3~25.0 mg/mL;进一步研究发现,SEM改变了细菌形态和膜结构。曹鑫明[63]在评估SEM对8种食品腐败菌抑制效果的过程中也发现,SEM破坏了细菌膜结构并增加了其通透性;进一步研究还发现,SEM能作用于细菌DNA复制的准备期来抑制细菌的复制,但对细菌DNA没有直接影响。综上所述,SEM发挥抗菌作用一方面通过对细菌的生物膜造成破坏,另一方面通过影响细菌的分裂周期来抑制细菌的复制。

2.5 保护肠道屏障

肠道屏障功能是维持机体健康的重要生理机制,能够防止有害物质从肠腔进入血液循环或其他组织器官,同时允许营养物质的正常吸收。研究发现,瑞士白鼠在接受15 Gy全身γ射线照射前通过腹腔注射给予50 mg/kg BW剂量的SEM能够维持空肠绒毛高度接近正常水平,而100 mg/kg BW剂量的SEM减少了空肠组织中炎症细胞和死亡细胞的数量[64]。在Khan等[65]的研究中也显示,SEM预处理减少了辐射诱导的胃肠道损伤,增加了隐窝细胞数量以及绒毛的数量和长度。短链脂肪酸(short chain fatty acids,SCFAs)能够为肠上皮细胞提供能量,调节其增殖、分化以及肠内分泌细胞等亚群的功能,从而影响肠道蠕动并增强肠道屏障功能[66]。已有证据表明,在高脂饮食中添加0.05%的SEM,可显著提高野生型肥胖小鼠粪便中的SCFAs含量,并显著提高芽孢杆菌、乳杆菌等有益菌的相对丰度[67]。在另一项研究中也显示,SEM能提高肠道中双歧杆菌、阿克曼菌等有益菌的相对丰度[68]。由此可知,SEM能够维持肠道屏障的完整性,调节肠道微生物的群落结构,并提高肠道中有益菌的相对丰度,从而保护肠道屏障。

2.6 抗肿瘤作用

SEM的抗肿瘤作用涉及细胞凋亡、能量代谢、血管生成等方面。细胞凋亡可以通过外源性和内源性2条途径。Fas受体是一种死亡受体,在外源性途径中发挥关键作用,Fas配体(Fas ligand,FasL)则是它的配体;内源性途径则主要通过线粒体释放膜间隙中的电子传递蛋白细胞色素C来启动细胞凋亡[69]。半胱氨酸天冬氨酸蛋白酶(cysteinyl aspartate specific protease,Caspase)和B细胞淋巴瘤-2(B-cell lymphoma-2,Bcl-2)家族蛋白是细胞凋亡过程中的2类关键蛋白,Caspase-8和Caspase-3分别在细胞凋亡的启动和执行阶段发挥作用,Bcl-2家族蛋白则包括抗凋亡蛋白Bcl-2以及促凋亡蛋白B细胞淋巴瘤-2相关X蛋白(B-cell lymphoma-2 related X protein,Bax)、B细胞淋巴瘤-2同源3相互作用结构域凋亡诱导蛋白(B-cell lymphoma-2 homology 3 interacting domain death agonist,Bid)[70]。有证据表明,70 mg/kg BW剂量的SEM显著减少了Ehrlich实体癌模型小鼠的肿瘤大小和重量[71]。SEM以剂量依赖性方式抑制人肝癌细胞(HepG2)的增殖,使细胞周期停滞在DNA复制期,并提高细胞凋亡率[72]。进一步研究发现,SEM通过内源性和外源性凋亡途径诱导细胞凋亡,在外源性凋亡途径中,SEM上调了Fas/FasL和Bid蛋白活性片段tBid的表达,并激活Caspase-8;在内源性途径中,SEM降低了线粒体膜电位以及抗凋亡蛋白Bcl-2的表达,促进了细胞色素C的释放和Caspase-3的激活,同时,SEM还显著抑制了HepG2的线粒体呼吸功能,降低了基础呼吸和最大呼吸能力,通过调节能量代谢来抑制癌细胞的生长和增殖[72]。血管生成因子(vascular endothelial growth factor,VEGF)在肿瘤的形成和发展中起关键作用,是抗肿瘤治疗的重要靶点,而VEGFR-2是VEGF的主要受体[73]。Elzanaty等[74]研究表明,SEM能够显著抑制VEGFR-2的表达,从而抑制肿瘤的血管生成。

3 SEM在畜禽生产中的应用

SEM作为一种天然的植物提取物,具有多种生物学功能,但其在畜禽生产中的应用还不够广泛。Ismail等[75]报道,SEM与α-生育酚的组合在减缓辐射和未辐射碎牛肉的脂质氧化方面非常有效,但也对肉色产生不利影响。Sallam等[76]研究表明,0.5 g/kg SEM处理的肉丸需氧菌落总数显著降低,并随着储存时间的延长,在第15天和之后完全抑制了肠杆菌科的生长,SEM作为天然抗菌剂,能有效抑制肉丸中多种食源性病原体和腐败细菌的生长,从而延长肉丸的货架期,并提高其安全性。王萍萍等[77]研究显示,在猪精液稀释液中添加5.5 mg/L的SEM可以显著降低ROS和MDA含量,提高精液品质及抗氧化能力。有证据表明,SEM可由芝麻烘烤过程中芝麻素的降解产生的[78],因此,经过热处理的芝麻制品及副产物中具有一定的SEM含量。研究显示,在饲粮中使用芝麻油对雄性肉鸡生长性能、血液代谢物含量和胃肠健康有积极影响[79]。Al-Daraji等[80]研究发现,补充1%芝麻油显著改善了鹌鹑蛋品质。而在乳山羊饲粮中添加10%的芝麻油粕替代豆粕,显著降低了山羊乳中饱和脂肪酸和不饱和脂肪酸的比例以及动脉粥样硬化指数值,可能是芝麻油中的抗氧化成分在发挥作用[81]。有研究显示,用甲醛处理的芝麻粕替代12.5%的豆粕可以提高泌乳山羊的营养摄入量、牛奶产量和乳成分,同时改善瘤胃发酵特性[82]。有证据表明,芝麻粕可以部分替代豆粕,且在不超过8%的添加水平下,对羔羊生长和肉质没有负面影响,同时降低了饲养成本[83]。在肉鸡饲粮中添加12%的烤芝麻壳,提高了饲粮摄入量,改善了生长性能[84]。而在奶牛饲粮中添加10%和20%的芝麻籽粕可以显著提高奶牛的产奶量、乳成分和经济效益,同时对奶牛健康无负面影响[85]

4 小结

SEM作为一种天然的植物提取物,展现出多种生理功能,显示了在畜禽生产中的应用前景。然而,目前关于SEM在畜禽生产中的研究和应用相对有限。因此,迫切需要进一步研究SEM在不同畜禽种类中的适宜添加剂量、作用效果及机制,为SEM在畜禽生产中应用奠定理论基础。
[1]
LOW C X, TAN L T H, AB MUTALIB N S, et al. Unveiling the impact of antibiotics and alternative methods for animal husbandry:a review[J]. Antibiotics, 2021, 10(5):578.

[2]
佚名. 中华人民共和国农业农村部公告第194号[J]. 浙江畜牧兽医, 2020, 45(1):28-29.

Anon. Announcement No.194 of the Ministry of Agriculture and Rural Affairs of the People’s Republic of China[J]. Zhejiang Animal Husbandry and Veterinary, 2020, 45(1):28-29. (in Chinese)

[3]
HUANG J N, QI S N, SUN Q, et al. Antioxidant capacity of sesamol in Caenorhabditis elegans model system[J]. Food Production,Processing and Nutrition, 2024, 6(1):7.

[4]
MAJDALAWIEH A F, AHARI S H, YOUSEF S M, et al. Sesamol:a lignan in sesame seeds with potent anti-inflammatory and immunomodulatory properties[J]. European Journal of Pharmacology, 2023,960:176163.

[5]
YANG Y, QU Y, LV X Q, et al. Sesamol supplementation alleviates nonalcoholic steatohepatitis and atherosclerosis in high-fat,high carbohydrate and high-cholesterol diet-fed rats[J]. Food & Function, 2021, 12(19):9347-9359.

[6]
WU M J, DONG Q L, SONG X, et al. Effective combination of nisin and sesamol against Listeria monocytogenes[J]. LWT, 2023,176:114546.

[7]
蔡雅慧, 李艳平, 魏晓楠. 芝麻酚的生物学功能及其在抗肿瘤中作用[J]. 中国生物化学与分子生物学报, 2025, 41(1):105-111.

DOI

CAI Y H, LI Y P, WEI X N. Biological functions of sesamol and its role in antitumor activity[J]. Chinese Journal of Biochemistry and Molecular Biology, 2025, 41(1):105-111. (in Chinese)

[8]
储传奇. 芝麻酚改善高脂膳食诱导的肥胖及肠道屏障损伤的作用机制研究[D]. 硕士学位论文. 杨凌: 西北农林科技大学, 2018.

CHU C Q. Research on the mechanism of sesamol in improving obesity and intestinal barrier damage induced by high-fat diet[D]. Master’s Thesis. Yangling: Northwest A&F University, 2018. (in Chinese)

[9]
ZHOU S Y, ZOU H Y, HUANG G L, et al. Preparations and antioxidant activities of sesamol and it’s derivatives[J]. Bioorganic & Medicinal Chemistry Letters, 2021,31:127716.

[10]
SHAH A, LOBO R, KRISHNADAS N, et al. Sesamol and health-a comprehensive review[J]. Indian Journal of Pharmaceutical Education and Research, 2019, 53(Suppl.2):S28-S42.

[11]
MAJDALAWIEH A F, MANSOUR Z R. Sesamol,a major lignan in sesame seeds (Sesamum indicum):anti-cancer properties and mechanisms of action[J]. European Journal of Pharmacology, 2019,855:75-89.

[12]
JAYARAJ P, NARASIMHULU C A, RAJAGOPALAN S, et al. Sesamol:a powerful functional food ingredient from sesame oil for cardioprotection[J]. Food & Function, 2020, 11(2):1198-1210.

[13]
BETTERIDGE D J. What is oxidative stress?[J]. Metabolism, 2000, 49(2 Suppl.1):3-8.

[14]
SMARZEWSKA S, GUZIEJEWSKI D, ULLAH N, et al. Electrochemical evaluation of free radical scavenging activity of sesamol[J]. Journal of the Electrochemical Society, 2023, 170(5):055502.

[15]
JOSHI R, KUMAR M S, SATYAMOORTHY K, et al. Free radical reactions and antioxidant activities of sesamol:pulse radiolytic and biochemical studies[J]. Journal of Agricultural and Food Chemistry, 2005, 53(7):2696-2703.

[16]
HIRAMOTO K, OJIMA N, SAKO K, et al. Effect of plant phenolics on the formation of the spin-adduct of hydroxyl radical and the DNA Strand breaking by hydroxyl radical[J]. Biological and Pharmaceutical Bulletin, 1996, 19(4):558-563.

PMID

[17]
BEHESHTIMANESH Z, RAJAEI Z. Neuroprotective effects of sesamol against LPS-induced spatial learning and memory deficits are mediated via anti-inflammatory and antioxidant activities in the rat brain[J]. Avicenna Journal of Phytomedicine, 2023, 13(2):213-222.

DOI PMID

[18]
CARBONE M C, TATONE C, DELLE MONACHE S, et al. Antioxidant enzymatic defences in human follicular fluid:characterization and age-dependent changes[J]. Molecular Human Reproduction, 2003, 9(11):639-643.

[19]
VON MENGDEN L, KLAMT F, SMITZ J. Redox biology of human cumulus cells:basic concepts,impact on oocyte quality,and potential clinical use[J]. Antioxidants & Redox Signaling, 2020, 32(8):522-535.

[20]
WEYDERT C J, CULLEN J J. Measurement of superoxide dismutase,catalase and glutathione peroxidase in cultured cells and tissue[J]. Nature Protocols, 2010, 5(1):51-66.

[21]
RUANKHAM W, SUWANJANG W, WONGCHITRAT P, et al. Sesamin and sesamol attenuate H2O2-induced oxidative stress on human neuronal cells via the SIRT1-SIRT3-FOXO3a signaling pathway[J]. Nutritional Neuroscience, 2021, 24(2):90-101.

[22]
HEMALATHA G, PUGALENDI K V, SARAVANAN R. Modulatory effect of sesamol on DOCA-salt-induced oxidative stress in uninephrectomized hypertensive rats[J]. Molecular and Cellular Biochemistry, 2013, 379(1/2):255-265.

[23]
赵卫平, 张红, 邱嵘, 等. 碳离子全身辐照对小鼠血清及肝脏中超氧化物歧化酶活性、丙二醛含量和脑组织中还原性谷胱甘肽浓度的影响[J]. 辐射研究与辐射工艺学报, 2007, 25(1):33-36.

ZHAO W P, ZHANG H, QIU R, et al. Superoxide dismutase activity and maleic dialdehyde content in serum and liver and glutathione level in brain of 12C6+ ions-irradiated mice[J]. Journal of Radiation Research and Radiation Processing, 2007, 25(1):33-36. (in Chinese)

[24]
赵培均, 王田林, 谢珊珊, 等. 芝麻酚通过调节SLC7A11/GPX4/ACSL4轴抑制Aβ1-42诱导的PC12细胞铁死亡[J]. 食品科学, 2025, 46(10):139-146.

ZHAO P J, WANG T L, XIE S S, et al. Sesamol inhibits Aβ1-42-induced ferroptosis in PC12 cells by regulating the SLC7A11/GPX4/ACSL4 axis[J]. Food Science, 2025, 46(10):139-146. (in Chinese)

[25]
LIOU C J, CHEN Y L, YU M C, et al. Sesamol alleviates airway hyperresponsiveness and oxidative stress in asthmatic mice[J]. Antioxidants, 2020, 9(4):295.

[26]
LI L R, DONG H, SONG E Q, et al. Nrf2/ARE pathway activation,HO-1 and NQO1 induction by polychlorinated biphenyl quinone is associated with reactive oxygen species and PI3K/AKT signaling[J]. Chemico-Biological Interactions, 2014,209:56-67.

[27]
谢允东, 王小平, 何世鹏. 芝麻酚对模型小鼠肝损伤的改善作用[J]. 中国药业, 2021, 30(18):37-41.

XIE X D, WANG X P, HE S P, et al. Improvement effect of sesamol on liver injury in model mice[J]. China Pharmaceuticals, 2021, 30(18):37-41. (in Chinese).

[28]
任波. 芝麻酚调控系统性氧化应激及Nrf2/ARE抗氧化防御信号的应答分子机制研究[D]. 硕士学位论文. 杨凌: 西北农林科技大学, 2017.

REN B. Effects and mechanism of sesamol on systemic oxidative stress and NRF2/ARE antioxidant defense signaling pathways[D]. Master’s Thesis. Yangling: Northwest A&F University, 2017. (in Chinese)

[29]
陆志城. 环氧化酶及其研究进展[J]. 广东药学, 2004, 14(3):65-69.

LU Z C. Cyclooxygenase and its research progress[J]. Guangdong Pharmaceutical Journal, 2004, 14(3):65-69. (in Chinese)

[30]
ZHAO B T, XIA B, LI X H, et al. Sesamol supplementation attenuates DSS-induced colitis via mediating gut barrier integrity,inflammatory responses,and reshaping gut microbiome[J]. Journal of Agricultural and Food Chemistry, 2020, 68(39):10697-10708.

[31]
蒋波, 楚正绪. 一氧化氮与炎症[J]. 国外医学(生理、病理科学与临床分册), 1998(1):44-47.

JIANG B, CHU Z X. Nitric oxide and inflammation[J]. Foreign Medical Science (Section of Pathophysiology and Clinical Medicine), 1998(1):44-47. (in Chinese)

[32]
杨季云, 张思仲, 郭红, 等. 肿瘤坏死因子α通过激活NF-κB信号通路加快肝细胞周期进程[J]. 生物化学与生物物理进展, 2007, 34(6):604-610.

YANG J Y, ZHANG S Z, GUO H, et al. TNF-α promotes cell cycle progression by activating NF-κB signal pathway in hepatic cell line L-02[J]. Progress in Biochemistry and Biophysics, 2007, 34(6):604-610. (in Chinese)

[33]
盛冰莹. 芝麻油加工过程中芝麻酚的形成规律及抗炎活性研究[D]. 硕士学位论文. 郑州: 河南工业大学, 2023.

SHENG B Y. Study on the formation pattern of sesamol and anti-inflammatory activity during the processing of sesame oil[D]. Master’s Thesis. Zhengzhou: Henan University of Technology, 2023. (in Chinese)

[34]
LIU T, ZHANG L Y, JOO D, et al. NF-κB signaling in inflammation[J]. Signal Transduction and Targeted Therapy, 2017,2:17023.

[35]
陈雪, 刘学波, 王雨萱. 芝麻酚对小鼠银屑病样炎症的抑制作用[J]. 食品与机械, 2023, 39(6):166-172.

CHEN X, LIU X B, WANG Y X. Inhibition of psoriasis-like inflammation in mice by sesamol[J]. Food & Machinery, 2023, 39(6):166-172. (in Chinese)

[36]
于渝梦. 芝麻林素转化为芝麻酚的反应机制及芝麻酚抗炎活性研究[D]. 硕士学位论文. 郑州: 河南工业大学, 2024.

YU Y M. Study on the reaction mechanism of sesamolin transforms into sesamol and the anti-inflammatory activity of sesamo[D]. Master’s Thesis. Zhengzhou: Henan University of Technology, 2024. (in Chinese)

[37]
KIM J, YANG G, KIM Y, et al. AMPK activators:mechanisms of action and physiological activities[J]. Experimental & Molecular Medicine, 2016, 48(4):e224.

[38]
DAGON Y, MANTZOROS C S, KIM Y B. AMPK↔SIRT1:from a signaling network to a combination drug[J]. Metabolism-Clinical and Experimental, 2016, 65(11):1692-1694.

[39]
刘瞩, 程明慧, 张劝劝, 等. 芝麻酚通过AMPK信号通路调控巨噬细胞极化减轻脂肪组织炎症[J]. 中国药理学通报, 2023, 39(11):2082-2088.

LIU Z, CHENG M H, ZHANG Q Q, et al. Sesamol reduces adipose tissue inflammation by regulating macrophage polarization through AMPK signaling pathway[J]. Chinese Pharmacological Bulletin, 2023, 39(11):2082-2088. (in Chinese)

[40]
FENG X C, CHEN X H, ZAEEM M, et al. Sesamol attenuates neuroinflammation by regulating the AMPK/SIRT1/NF-κB signaling pathway after spinal cord injury in mice[J]. Oxidative Medicine and Cellular Longevity, 2022,2022:8010670.

[41]
QIN H, XU H Y, YU L, et al. Sesamol intervention ameliorates obesity-associated metabolic disorders by regulating hepatic lipid metabolism in high-fat diet-induced obese mice[J]. Food & Nutrition Research, 2019,63:3637.

[42]
孔祥, 华强, 姚新明, 等. 芝麻酚调控巨噬细胞极化改善肥胖小鼠脂肪组织炎症及胰岛素抵抗[J]. 中国临床药理学与治疗学, 2020, 25(7):728-733.

KONG X, HUA Q, YAO X M, et al. Sesamol improves inflammation and insulin resistance in adipose tissue of obese mice by regulating macrophage polarization[J]. Chinese Journal of Clinical Pharmacology and Therapeutics, 2020, 25(7):728-733. (in Chinese)

[43]
SHI L K, KARRAR E, LIU R J, et al. Comparative effects of sesame lignans (sesamin,sesamolin,and sesamol) on oxidative stress and lipid metabolism in steatosis HepG2 cells[J]. Journal of Food Biochemistry, 2022, 46(8):e14180.

[44]
MONTAIGNE D, BUTRUILLE L, STAELS B. PPAR control of metabolism and cardiovascular functions[J]. Nature Reviews Cardiology, 2021, 18(12):809-823.

DOI PMID

[45]
WAKIL S J, ABU-ELHEIGA L A. Fatty acid metabolism:target for metabolic syndrome[J]. Journal of Lipid Research,2009,50:S138-S143.

[46]
CLARKE S D. Regulation of fatty acid synthase gene expression:an approach for reducing fat accumulation[J]. Journal of Animal Science, 1993, 71(7):1957-1965.

[47]
MAUVOISIN D, MOUNIER C. Hormonal and nutritional regulation of SCD1 gene expression[J]. Biochimie, 2011, 93(1):78-86.

[48]
SHI L K, KARRAR E, WANG X G. Sesamol ameliorates hepatic lipid accumulation and oxidative stress in steatosis HepG2 cells via the PPAR signaling pathway[J]. Journal of Food Biochemistry, 2021, 45(11):e13976.

[49]
乔青莲. 芝麻酚对高脂高果糖诱导的肥胖及胰岛素抵抗的调控作用与机制研究[D]. 硕士学位论文. 杨凌: 西北农林科技大学, 2017.

QIAO Q L. Preventive effects of sesamol on high fat and high fructose-induced obesity and insulin resistance[D]. Master’s Thesis. Yangling: Northwest A&F University, 2017. (in Chinese)

[50]
HU M M, CHEN J H, ZHANG Q Q, et al. Sesamol counteracts on metabolic disorders of middle-aged alimentary obese mice through regulating skeletal muscle glucose and lipid metabolism[J]. Food & Nutrition Research, 2022,66:8231.

[51]
ALTHAHER A R. An overview of hormone-sensitive lipase (HSL)[J]. The Scientific World Journal, 2022,2022:1964684.

[52]
JEOUNG N H, HARRIS R A. Role of pyruvate dehydrogenase kinase 4 in regulation of blood glucose levels[J]. Korean Diabetes Journal, 2010, 34(5):274-283.

DOI PMID

[53]
DENTIN R, GIRARD J, POSTIC C. Carbohydrate responsive element binding protein (ChREBP) and sterol regulatory element binding protein-1c (SREBP-1c):two key regulators of glucose metabolism and lipid synthesis in liver[J]. Biochimie, 2005, 87(1):81-86.

[54]
VARGAS E, PODDER V,CARRILLO SEPULVEDA M A. Physiology,glucose transporter type 4[M]// StatPearlsInternet. Treasure Island (FL): StatPearls Publishing, 2025.

[55]
STEPHENS M, LUDGATE M, REES D A. Brown fat and obesity:the next big thing?[J]. Clinical Endocrinology, 2011, 74(6):661-670.

[56]
LIN C, CHEN J H, HU M M, et al. Sesamol promotes browning of white adipocytes to ameliorate obesity by inducing mitochondrial biogenesis and inhibition mitophagy via β3-AR/PKA signaling pathway[J]. Food & Nutrition Research, 2021,65:7577.

[57]
KALINOVICH A V, DE JONG J M A, CANNON B, et al. UCP1 in adipose tissues:two steps to full browning[J]. Biochimie, 2017,134:127-137.

[58]
SEO Y J, JIN H, LEE K, et al. Cardamonin suppresses lipogenesis by activating protein kinase a-mediated browning of 3T3-L1 cells[J]. Phytomedicine, 2019,65:153064.

[59]
ZHANG J K, MIAO J, CHEN Z Q, et al. β3-adrenergic activation improves maternal and offspring perinatal outcomes in diet-induced prepregnancy obesity in mice[J]. Obesity, 2019, 27(9):1482-1493.

[60]
LEE D H, CHANG S H, YANG D K, et al. Sesamol increases Ucp1 expression in white adipose tissues and stimulates energy expenditure in high-fat diet-fed obese mice[J]. Nutrients, 2020, 12(5):1459.

[61]
LI Z S, WU M J, YAN H, et al. Antibacterial effect and possible mechanism of sesamol against foodborne pathogens[J]. Foods, 2024, 13(3):435.

[62]
YENN T W, HASHIM N F F M, SAA L L, et al. Antibacterial and antioxidant activities of Ghee Hiang sesame oil extract[J]. Malaysian Journal of Medicine & Health Sciences, 2023,19 (Suppl.9):75-81.

[63]
曹鑫明. 芝麻酚的抗氧化、抑菌活性及抑菌机理研究[D]. 硕士学位论文. 太原: 山西师范大学, 2018.

CAO X M. Study on antioxidant, antibacterial activity and antibacterial mechanism of sesamol[D]. Master’s Thesis. Taiyuan: Shanxi Normal University, 2018. (in Chinese)

[64]
PARIHAR V K, PRABHAKAR K R, VEERAPUR V P, et al. Effect of sesamol on radiation-induced cytotoxicity in Swiss albino mice[J]. Mutation Research, 2006, 611(1/2):9-16.

[65]
KHAN S, KUMAR A, ADHIKARI J S, et al. Protective effect of sesamol against 60Co γ-ray-induced hematopoietic and gastrointestinal injury in C57BL/6 male mice[J]. Free Radical Research, 2015, 49(11):1344-1361.

[66]
MARTIN-GALLAUSIAUX C, MARINELLI L, BLOTTIÈRE H M, et al. SCFA:mechanisms and functional importance in the gut[J]. Proceedings of the Nutrition Society, 2021, 80(1):37-49.

[67]
YUAN T, CHU C Q, SHI R B, et al. ApoE-dependent protective effects of sesamol on high-fat diet-induced behavioral disorders:regulation of the microbiome-gut-brain axis[J]. Journal of Agricultural and Food Chemistry, 2019, 67(22):6190-6201.

[68]
WANG L, CHEN W X, TIAN Y J, et al. Preventive effects of sesamol on deep-frying oil-induced liver metabolism disorders by altering gut microbiota and protecting gut barrier integrity[J]. Molecular Nutrition & Food Research, 2022, 66(9):e2101122.

[69]
LAWEN A. Apoptosis-an introduction[J]. BioEssays, 2003, 25(9):888-896.

DOI PMID

[70]
SWANTON E, SAVORY P, COSULICH S, et al. BCL-2 regulates a caspase-3/caspase-2 apoptotic cascade in cytosolic extracts[J]. Oncogene, 1999, 18(10):1781-1787.

DOI PMID

[71]
ABD ELRAZIK N A, EL-MESERY M, EL-KAREF A, et al. Sesamol upregulates death receptors and acts as a chemosensitizer in solid Ehrlich carcinoma model in mice[J]. Nutrition and Cancer, 2022, 74(1):250-264.

[72]
LIU Z G, REN B, WANG Y H, et al. Sesamol induces human hepatocellular carcinoma cells apoptosis by impairing mitochondrial function and suppressing autophagy[J]. Scientific Reports, 2017,7:45728.

[73]
NEUFELD G, COHEN T, GENGRINOVITCH S, et al. Vascular endothelial growth factor (VEGF) and its receptors[J]. The FASEB Journal, 1999, 13(1):9-22.

[74]
ELZANATY K A, OMRAN G A, ELMAHALLAWY E K, et al. Design and optimization of sesamol nanosuspensions to potentiate the anti-tumor activity of epirubicin against Ehrlich solid carcinoma-bearing mice[J]. Pharmaceutics, 2024, 16(7):937.

[75]
ISMAIL H A, LEE E J, KO K Y, et al. Effect of antioxidant application methods on the color,lipid oxidation,and volatiles of irradiated ground beef[J]. Journal of Food Science, 2009, 74(1):C25-C32.

[76]
SALLAM K I, ABD-ELGHANY S M, IMRE K, et al. Ensuring safety and improving keeping quality of meatballs by addition of sesame oil and sesamol as natural antimicrobial and antioxidant agents[J]. Food Microbiology, 2021,99:103834.

[77]
王萍萍, 王根盛, 季愚智, 等. 芝麻酚对猪精液17 ℃保存效果的影响[J]. 中国畜牧杂志, 2024, 60(8):329-334.

WANG P P, WANG G S, JI Y Z, et al. Effect of sesamol on preservation of boar semen at 17 ℃[J]. Chinese Journal of Animal Science, 2024, 60(8):329-334. (in Chinese)

[78]
LEE S W, JEUNG M K, PARK M H, et al. Effects of roasting conditions of sesame seeds on the oxidative stability of pressed oil during thermal oxidation[J]. Food Chemistry, 2010, 118(3):681-685.

[79]
AGAH M J, GOLIAN A, NASSIRI-MOGHADDAM H, et al. Effect of dietary supplementation of sesame (Sesamum indicum L.) oil and/or Α-tocopheryl acetate on performance,intestinal morphology and blood metabolites in male broiler chickens[J]. Research on Animal Production, 2016, 6(12):30-41.

[80]
AL-DARAJI H J, AL-MASHADANI H A, AL-HAYANI W K, et al. Effect of the supplementation of the laying quails ration with sesame (Sesamum indicum) seeds and oil on egg quality traits[J]. International Journal of Applied Biology and Pharmaceutical Technology, 2012, 3(4):54-63.

[81]
MITSIOPOULOU C, KARAISKOU C, SIMONI M, et al. Influence of dietary sesame meal,vitamin E and selenium supplementation on milk production,composition,and fatty acid profile in dairy goats[J]. Livestock Science, 2021,244:104336.

[82]
FIROZI F, DAYANI O, TAHMASBI R, et al. Feeding formaldehyde-treated sesame meal to lactating murciano-granadina goats:implications on milk yield and composition,digestibility,rumen fermentation,and blood metabolites[J]. Spanish Journal of Agricultural Research, 2024, 22(1):e0602.

[83]
OBEIDAT B S, ABDULLAH A Y, MAHMOUD K Z, et al. Effects of feeding sesame meal on growth performance,nutrient digestibility,and carcass characteristics of Awassi lambs[J]. Small Ruminant Research, 2009, 82(1):13-17.

[84]
MAHMOUD K Z, OBEIDAT B S, ISHMAIS M A. Roasted sesame hulls improve broiler performance without affecting carcass characteristics[J]. Italian Journal of Animal Science, 2015, 14(3):3957.

[85]
QUSSAY Z, ESSAM A J, HUSSAIN A S, et al. Milk production,composition and economic efficiency and some blood parameters of local Friesian dairy cows fed sesame seed meal[J]. Kufa Journal for Veterinary Medical Sciences, 2015, 6(2):205-215.

Outlines

/