RESEARCH PAPER

Effects of Caragana korshinskii Tannins on Growth Performance, Nutrient Apparent Digestibility, Small Intestinal Morphology and Antioxidant Function of Fattening Lambs Fed High-Concentrate Diets

  • LI Hui ,
  • NIU Xiaoyu ,
  • CHEN Zhiyu ,
  • WANG Yaning ,
  • XING Yuanyuan ,
  • LI Dabiao , *
Expand
  • Key Laboratory of Animal Nutrition and Feed Science at Universities of Inner Mongolia Autonomous Region, College of Animal Science, Inner Mongolia Agricultural University, Hohhot 010018, China
*professor, E-mail:

Received date: 2025-01-03

  Online published: 2025-08-14

Abstract

This experiment was conducted to investigate the effects of Caragana korshinskii tannins (CKT) on growth performance, nutrient apparent digestibility, small intestinal morphology and antioxidant function of fattening lambs fed high-concentrate diets. Twenty-four 3-month-old Dorper×Mongolian crossbred male lambs were randomly divided into 3 groups with 8 replicates per group and 1 lamb per replicate. Lambs in control group (CON group) were fed a diet with a concentrate to forage ratio of 3∶7, those in high-concentrate group (HC group) were fed a high-concentrate diet with a concentrate to forage ratio of 7∶3, and those in CKT group were fed a diet supplemented with 2 g/kg CKT in the high-concentrate diet. The pre-trial period lasted for 15 days, and the formal trial period lasted for 60 days. The results showed as follows: 1) compared with CON group, the average daily gain (ADG) of lambs in HC group was significantly increased (P<0.05), while the feed-to-gain ratio (F/G) was significantly decreased (P<0.05). 2) Compared with CON group, the apparent digestibility of crude protein (CP) and ether extract (EE) of lambs in HC group was significantly increased (P<0.05). 3) Compared with CON group, the villus height (VH) and villus height/crypt depth (V/C) in ileum of lambs in HC group were significantly decreased (P<0.05). Compared with HC group, the VH in ileum of lambs in CKT group was significantly increased (P<0.05), the crypt depth (CD) in jejunum and ileum was significantly decreased (P<0.05), and the V/C in duodenum and ileum was significantly increased (P<0.05). 4) Compared with CON group, the total antioxidant capacity (T-AOC) in jejunum of lambs in HC group was significantly decreased (P<0.05), while the malondialdehyde (MDA) content in ileum was significantly increased (P<0.05); moreover, the mRNA relative expression levels of NAD(P)H: quinone oxidoreductase 1 (NQO1) and heme oxygenase-1 (HO-1) in duodenum, NQO1 in jejunum and superoxide dismutase 1 (SOD1) in ileum were significantly decreased (P<0.05). Compared with HC group, the MDA content in ileum of lambs in CKT group was significantly decreased (P<0.05), and the mRNA relative expression levels of catalase (CAT) in duodenum, glutathione peroxidase 1 (GPx1) in jejunum and SOD1 in ileum were significantly increased (P<0.05). In conclusion, high-concentrate diet supplemented with 2 g/kg CKT can improve the antioxidant function of fattening lambs by enhancing the morphological structure of small intestine, regulating MDA content in small intestine, and increasing the expression of genes related to antioxidant, while not affecting their growth performance, thereby alleviating the oxidative damage to small intestine caused by high-concentrate diet and promoting overall health.

Cite this article

LI Hui , NIU Xiaoyu , CHEN Zhiyu , WANG Yaning , XING Yuanyuan , LI Dabiao . Effects of Caragana korshinskii Tannins on Growth Performance, Nutrient Apparent Digestibility, Small Intestinal Morphology and Antioxidant Function of Fattening Lambs Fed High-Concentrate Diets[J]. Chinese Journal of Animal Nutrition, 2025 , 37(8) : 5342 -5353 . DOI: 10.12418/CJAN2025.434

近年来,我国畜牧业发展势头强劲,肉羊养殖业正逐步由小规模饲养迈向高效益的规模化舍饲养殖新时代。然而,随着舍饲与半舍饲模式下肉羊数量的急剧攀升,饲粮搭配的科学性与营养均衡性成为制约养殖效率的关键因素。肉羊营养摄入不平衡时,易引发营养代谢疾病和肉品质下降,最终造成经济效益下滑。为此,养殖者通常对反刍动物采用高精料饲粮进行育肥。然而,动物长期采食高精料饲粮会对机体造成不利影响,诱发亚急性瘤胃酸中毒(SARA)[1]、肠黏膜受损[2]、肠道氧化应激[3]等问题,进而引发全身系统性疾病。小肠是营养物质消化吸收的主要场所,也是抵御毒素入侵的重要屏障[4]。小肠上皮由单层柱状上皮细胞构成,极易受到细菌等毒素的刺激[5]。当机体受到内部或外部刺激时,细胞内外会产生大量自由基。若自由基含量超过机体自身清除能力,便会大量堆积,打破机体氧化与抗氧化系统间的动态平衡,进而导致机体组织DNA、蛋白质、脂肪结构损伤,当这种损伤不能恢复时,机体就会发生氧化损伤[6]
单宁属于多酚类物质,广泛存在于植物的根、茎、皮、叶和果实中,根据其结构被分为水解单宁(包括没食子单宁、鞣花单宁、复杂单宁)和缩合单宁[7-8]。由于单宁具有涩味,会降低动物的采食量,因此曾被视为“抗营养因子”。然而,近年来为了改善动物的免疫与抗氧化功能,在饲粮中添加适量植物单宁已成为一种重要的营养调控手段。单宁的酚羟基结构使其具有清除自由基的能力[9]。Pelegrin-Valls等[10]研究发现,饲喂富含缩合单宁的红豆草饲粮可显著提高羔羊回肠过氧化氢酶(CAT)活性和谷胱甘肽过氧化物酶(GPx)2的mRNA相对表达量。Guo等[11]研究发现,在断奶仔猪饲粮中添加400 mg/kg苹果多酚,能显著提高空肠总抗氧化能力(T-AOC)和总超氧化物歧化酶(T-SOD)活性,并显著上调空肠NAD(P)H:醌氧化还原酶1(NQO1)、血红素加氧酶-1(HO-1)和核因子红细胞2相关因子2(Nrf2)的mRNA相对表达量。Yu等[12]研究发现,饲粮中添加0.1%单宁酸可显著降低断奶仔猪回肠丙二醛(MDA)含量。本课题组前期研究表明,高精料饲粮中添加2 g/kg柠条单宁(Caragana korshinskii tannins,CKT)能够显著提高羔羊血清免疫及抗氧化能力[13]。基于此,本试验以育肥羔羊为研究对象,旨在探讨高精料饲粮中添加2 g/kg CKT对其生长性能、营养物质表观消化率、小肠形态结构及抗氧化功能的影响,以期为CKT作为饲料添加剂在反刍动物养殖中的开发与利用提供理论依据。

1 材料与方法

1.1 伦理声明

动物饲养试验在中国呼和浩特市内蒙古农业大学海流图试验基地进行。所有动物试验程序均遵循内蒙古农业大学实验动物福利和伦理委员会制定的伦理规范(批准号:NND2021098)。

1.2 试验设计与饲养管理

选取24只体重相近的3月龄杜蒙杂交公羔,随机分为3组,每组8个重复,每个重复1只羊。对照组(CON组)饲喂精粗比为3∶7的饲粮,高精料组(HC组)饲喂精粗比为7∶3的高精料饲粮,CKT组饲喂在高精料饲粮中添加2 g/kg CKT的饲粮。试验期75 d,其中预试期15 d,正试期60 d。
预试期前对羊舍进行消毒,对试验羊进行编号、称重并随机分组。同时对试验羊进行体内、体外驱虫。正试期间,每天饲喂2次(08:00和16:00),饲喂时,先将CKT与少量饲粮混合后投喂,待羔羊采食完毕,再将剩余饲粮全部倒入饲槽。羊只自由采食和饮水,保持羊舍通风良好、温度适宜及环境清洁卫生。

1.3 试验饲粮

CKT由内蒙古农业大学动物科学学院,内蒙古自治区高校动物营养与饲料科学重点实验室制备[14],缩合单宁含量为27.3%,由表没食子儿茶素、儿茶素、没食子酰表没食子儿茶素、表儿茶素、没食子儿茶素、没食子酰表儿茶素和儿茶素没食子酸酯组成,其摩尔比为1∶8.88∶2.65∶1.55∶1.92∶0.49∶0.14。参照《肉羊营养需要量》(NY/T 816—2021)配制精粗比分别为3∶7和7∶3的全混合颗粒饲粮,其组成及营养水平见表1
表1 饲粮组成及营养水平(风干基础)

Table 1 Composition and nutrient levels of diets (air-dry basis) %

项目
Items
精粗比
Concentrate to forage ratio
3∶7 7∶3
原料Ingredients
燕麦草Oat grass 31.00
苜蓿干草Alfalfa hay 29.00
向日葵壳Sunflower husk 10.00 30.00
玉米Corn 15.00 39.00
玉米皮Corn bran 2.00 8.00
大豆粕Soybean meal 7.50 13.50
菜籽粕Rapeseed meal 3.00 6.00
石粉Limestone 1.00
磷酸氢钙CaHPO4 1.00 1.00
食盐NaCl 0.50 0.50
预混料Premix1) 1.00 1.00
合计Total 100.00 100.00
营养水平Nutrient levels2)
代谢能ME/(MJ/kg) 7.86 10.04
干物质DM 96.22 92.90
粗蛋白质CP 15.47 16.57
粗脂肪EE 4.96 6.66
粗灰分Ash 12.08 7.55
中性洗涤纤维NDF 46.90 30.57
酸性洗涤纤维ADF 28.57 16.75
钙Ca 0.89 1.08
总磷TP 0.71 0.75

1)预混料为每千克饲粮提供The premix provided the following per kg of diets:Se 0.3 mg,Cu 6.5 mg,Fe 55 mg,I 0.5 mg,Mn 25 mg,Co 0.25 mg,VA 1 800 IU,VD 3 000 IU,VE 576 IU。
2)代谢能为根据《肉羊营养需要量》(NY/T 816—2021)所得计算值,其余为实测值。ME was a calculated value according to Nutrient Requirements of Meat-Type Sheep and Goat (NY/T 816—2021), while the others were measured values.

1.4 样品采集

采用四分法收集约500 g试验饲粮,置于-20 ℃冰箱中保存待测;正试期最后7 d,每天早晚通过直肠取粪法收集羔羊粪便各1次,并将其置于-20 ℃冰箱中保存,用于测定营养物质表观消化率。
正试期结束后,每组选取6只体重相近的羔羊进行屠宰。分离并结扎各肠段,将肠段中部纵向剖开,用剪刀分别剪取十二指肠、空肠和回肠各约1 cm肠段,置于4%多聚甲醛中固定,用于制作石蜡切片。最后,使用无菌刀片分别刮取十二指肠、空肠和回肠黏膜,各装入独立的2 mL冻存管中,放入液氮中暂存,随后转移至-80 ℃冰箱中保存,用于测定抗氧化指标及相关基因的表达。

1.5 指标测定与方法

1.5.1 生长性能

在正试期第1天和第60天,对所有羔羊进行称重,记为初重和末重,据此计算平均日增重(ADG),记录正试期间羔羊每天的采食量,计算平均日采食量(ADFI),并根据ADG和ADFI计算料重比(F/G)。

1.5.2 饲粮营养水平及营养物质表观消化率

饲粮和粪便样品中干物质(DM)含量参照GB/T 6435—2014测定;粗蛋白质(CP)含量参照GB/T 6432—2018测定;粗脂肪(EE)含量参照GB/T 6433—2006测定;粗灰分(Ash)含量参照GB/T 6438—2007测定,据此计算有机物(OM)含量;中性洗涤纤维(NDF)含量参照GB/T 20806—2022测定;酸性洗涤纤维(ADF)含量参照NY/T 1459—2022测定;酸不溶灰分(AIA)含量参照GB/T 23742—2009测定。饲粮钙(Ca)含量参照GB/T 6436—2018测定;总磷(TP)含量参照GB/T 6437—2018测定。
以AIA为内源指示剂进行营养物质表观消化率的计算,计算公式如下:

某营养物质表观消化率(%)=[1-(粪便中该营养物质含量/粪便中AIA含量)/(饲粮中该营养物质含量/饲粮中AIA含量)]×100。

1.5.3 小肠形态结构

固定好的小肠组织依次经不同梯度乙醇脱水、新鲜二甲苯透明处理和石蜡包埋后,切成5 μm厚的切片,进行苏木精-伊红(HE)染色,使用光学显微镜观察肠道形态结构。使用4×10倍显微镜(尼康,日本)及Image-Pro Plus 6.0软件对小肠绒毛结构进行观察分析,测量绒毛高度(VH)和隐窝深度(CD),并计算绒毛高度/隐窝深度(V/C)。

1.5.4 小肠抗氧化指标

采用南京建成生物工程研究所生产的试剂盒测定十二指肠、空肠和回肠中GPx、T-SOD、CAT活性,MDA含量及T-AOC。

1.5.5 小肠抗氧化相关基因表达

使用RNAsio Plus(TaKaRa,日本)按照说明书从小肠组织中分离总RNA,采用NanoDrop ND-2000分光光度计(Thermal Scientific,加拿大)检测RNA浓度和纯度。通过2.0%琼脂糖凝胶电泳验证RNA完整性后,利用试剂盒的gDNA Eraser Premix去除基因组DNA,再使用Prime ScriptTM RT reagent Kit(TaKaRa,日本)将RNA反转录为cDNA。采用Tli Rnase H Plus Kit(TaKaRa,日本)进行实时荧光定量PCR(RT-qPCR),反应程序为:95 ℃预变性30 s;95 ℃变性5 s,60 ℃退火30 s(40个循环);95 ℃变性5 s,60 ℃退火1 min;50 ℃冷却30 s。目的基因包括CATGPx1、超氧化物歧化酶1(SOD1)、Nrf2、NQO1、HO-1,以β-肌动蛋白(β-actin)作为内参基因,采用2-△△Ct法计算目的基因的mRNA相对表达量。PCR所用引物序列见表2,引物设计通过NCBI网站完成,由华大基因股份有限公司合成。
表2 引物序列

Table 2 Primer sequences

基因
Genes
引物序列
Primer sequences (5'—3')
GenBank登录号
GenBank accession
number
退火温度
Annealing
temperature/℃
产物长度
Product
length/bp
过氧化氢酶
CAT
F:AGAGGAAACGCCTGTGTGAG
R:TGACACACATCCTCTGCCAC
XM_060400055.1 60 197
谷胱甘肽过氧化物酶1
GPx1
F:AACGTAGCATCGCTCTGAGG
R:CAAACTGGTTGCACGGGAAG
XM_004018462.5 60 115
超氧化物歧化酶1
SOD1
F:TTGGAGACCTGGGCAATGTG
R:CTGCCCAAGTCATCTGGTCT
NM_001145185.2 60 142
核因子红细胞2相关因子2
Nrf2
F:GATGGACTTGGAGCTGCCC
R:GCTCATGCTCCTTCTGTCGT
XM_015093345.4 60 140
血红素加氧酶1
HO-1
F:CAGGCCACCAAGTGCTATGT
R:CAGGGCCTTCTGAGCAATCT
XM_027967703.3 60 141
NAD(P)H:醌氧化还原酶1
NQO1
F:TCTGGCCAATTCAGAGTGGCA
R:CAGGATCTGAACTCGGGCAT
XM_004015102.6 60 110
β-肌动蛋白
β-actin
F:TGAGGAGCACCCTGTG
R:GTCTCAAACATGATCTGGGT
NM_007393.5 60 84

1.6 数据统计与分析

试验数据采用SPSS 27.0软件进行单因素方差分析(one-way ANOVA),并采用Duncan氏法进行多重比较。结果以平均值和均值标准误(SEM)表示,P<0.05为差异显著。

2 结果

2.1 CKT对高精料育肥羔羊生长性能的影响

表3可知,与CON组相比,HC组羔羊ADG显著升高(P<0.05),F/G显著降低(P<0.05)。与HC组相比,CKT组羔羊初重、末重、ADG、ADFI和F/G均无显著变化(P>0.05)。
表3 CKT对高精料育肥羔羊生长性能的影响

Table 3 Effects of CKT on growth performance of fattening lambs fed high-concentrate diets

项目
Items
组别Groups SEM P
P-value
CON HC CKT
初重Initial weight/kg 31.31 30.23 30.18 0.321 0.279
末重Final weight/kg 39.28 41.80 41.75 0.503 0.052
平均日增重ADG/(kg/d) 0.13b 0.21a 0.19a 0.011 0.003
平均日采食量ADFI/(kg/d) 1.40 1.40 1.39 0.001 0.065
料重比F/G 9.34a 6.78b 7.32b 0.640 0.028

同行数据肩标无字母或相同字母表示差异不显著(P>0.05),不同小写字母表示差异显著(P<0.05)。下表同。

In the same row, values with no letter or the same letter superscripts mean no significant difference (P>0.05), while with different small letter superscripts mean significant difference (P<0.05). The same as below.

2.2 CKT对高精料育肥羔羊营养物质表观消化率的影响

表4可知,与CON组相比,HC组羔羊CP和EE表观消化率显著升高(P<0.05)。与HC组相比,CKT组羔羊DM、OM、CP、EE、ADF和NDF表观消化率均无显著变化(P>0.05)。
表4 CKT对高精料育肥羔羊营养物质表观消化率的影响

Table 4 Effects of CKT on nutrient apparent digestibility of fattening lambs fed high-concentrate diets %

项目
Items
组别Groups SEM P
P-value
CON HC CKT
干物质DM 78.08 83.69 80.25 1.106 0.109
有机物OM 83.56 86.85 83.44 1.145 0.410
粗蛋白质CP 53.28b 73.15a 71.35a 1.503 <0.001
粗脂肪EE 40.48b 75.00a 70.57a 2.362 <0.001
酸性洗涤纤维ADF 33.59 42.63 33.60 2.071 0.179
中性洗涤纤维NDF 37.96 45.46 36.06 2.232 0.251

2.3 CKT对高精料育肥羔羊小肠形态结构的影响

表5可知,与CON组相比,HC组羔羊回肠VH和V/C显著降低(P<0.05)。与HC组相比,CKT组羔羊回肠VH显著升高(P<0.05),空肠和回肠CD显著降低(P<0.05),十二指肠和回肠V/C显著升高(P<0.05)。
表5 CKT对高精料育肥羔羊小肠形态结构的影响

Table 5 Effects of CKT on small intestinal morphology of fattening lambs fed high-concentrate diets

项目
Items
组别Groups SEM P
P-value
CON HC CKT
十二指肠Duodenum
绒毛高度VH/μm 961.22 925.76 906.09 26.924 0.746
隐窝深度CD/μm 99.18 99.65 78.97 4.263 0.067
绒毛高度/隐窝深度V/C 9.78ab 8.93b 12.22a 0.603 0.045
空肠Jejunum
绒毛高度VH/μm 656.79 564.92 600.98 18.230 0.109
隐窝深度CD/μm 90.85a 93.57a 78.55b 2.838 0.038
绒毛高度/隐窝深度V/C 7.28 6.03 7.58 0.321 0.092
回肠Ileum
绒毛高度VH/μm 793.85a 551.08c 644.81b 29.981 <0.001
隐窝深度CD/μm 102.00a 102.02a 67.63b 5.980 0.005
绒毛高度/隐窝深度V/C 7.81b 5.40c 11.50a 0.778 <0.001
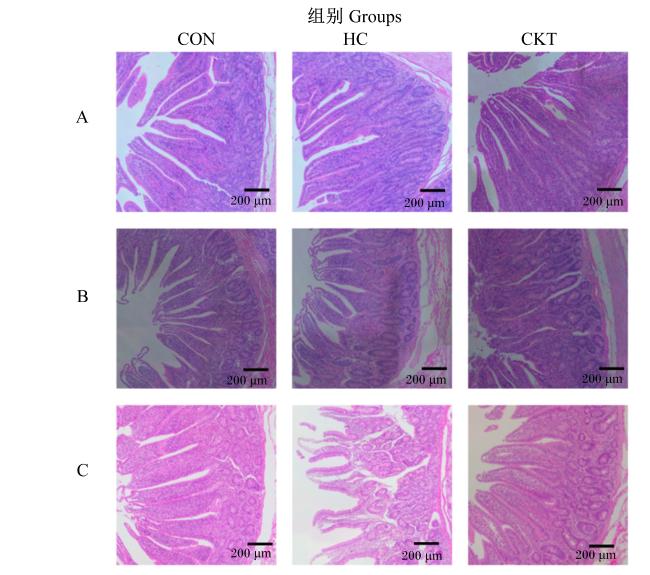
图1可知,与CON组相比,HC组羔羊十二指肠、空肠和回肠绒毛断裂,排列不整齐。与HC组相比,CKT组羔羊十二指肠、空肠和回肠形态结构受损有所改善。
图1 小肠形态结构

A:十二指肠 duodenum;B:空肠 jejunum;C:回肠 ileum。

Fig.1 Small intestinal morphology

2.4 CKT对高精料育肥羔羊小肠抗氧化指标的影响

表6可知,与CON组相比,HC组羔羊空肠T-AOC显著降低(P<0.05),回肠MDA含量显著升高(P<0.05)。与HC组相比,CKT组羔羊回肠MDA含量显著降低(P<0.05)。
表6 CKT对高精料育肥羔羊小肠抗氧化指标的影响

Table 6 Effects of CKT on small intestinal antioxidant indexes of fattening lambs fed high-concentrate diets

项目
Items
组别Groups SEM P
P-value
CON HC CKT
十二指肠Duodenum
过氧化氢酶CAT/(U/mg prot) 11.53 11.49 11.57 0.107 0.959
总抗氧化能力T-AOC/(mmol/g prot) 0.072 0.062 0.072 0.003 0 0.223
总超氧化物歧化酶T-SOD/(U/mg prot) 21.57 21.48 21.81 0.259 0.888
谷胱甘肽过氧化物酶GPx/(U/mg prot) 49.90 48.50 54.29 1.445 0.227
丙二醛MDA/(nmol/mg prot) 1.29 1.62 1.32 0.063 0.050
空肠Jejunum
过氧化氢酶CAT/(U/mg prot) 9.18 8.95 9.74 0.204 0.294
总抗氧化能力T-AOC/(mmol/g prot) 0.067a 0.057b 0.060ab 0.002 0 0.026
总超氧化物歧化酶T-SOD/(U/mg prot) 17.62 17.08 18.19 0.240 0.191
谷胱甘肽过氧化物酶GPx/(U/mg prot) 40.26 36.53 40.97 0.954 0.139
丙二醛MDA/(nmol/mg prot) 1.36 1.51 1.33 0.051 0.330
回肠Ileum
过氧化氢酶CAT/(U/mg prot) 4.98 4.87 5.19 0.121 0.601
总抗氧化能力T-AOC/(mmol/g prot) 0.070 0.053 0.053 0.004 0 0.100
总超氧化物歧化酶T-SOD/(U/mg prot) 18.77 18.63 19.13 0.389 0.885
谷胱甘肽过氧化物酶GPx/(U/mg prot) 54.39 42.95 49.43 2.283 0.127
丙二醛MDA/(nmol/mg prot) 0.98c 1.55a 1.29b 0.079 0.001

2.5 CKT对高精料育肥羔羊小肠抗氧化相关基因表达的影响

表7可知,与CON组相比,HC组羔羊十二指肠NQO1和HO-1、空肠NQO1、回肠SOD1的mRNA相对表达量显著降低(P<0.05)。与HC组相比,CKT组羔羊十二指肠CAT、空肠GPx1、回肠SOD1的mRNA相对表达量显著升高(P<0.05)。
表7 CKT对高精料育肥羔羊小肠抗氧化相关基因表达的影响

Table 7 Effects of CKT on small intestinal antioxidant-related gene expression of fattening lambs fed high-concentrate diets

项目
Items
组别Groups SEM P
P-value
CON HC CKT
十二指肠Duodenum
过氧化氢酶CAT 0.97b 0.71b 1.59a 0.131 0.009
谷胱甘肽过氧化物酶1 GPx1 1.02 0.88 0.93 0.057 0.624
超氧化物歧化酶1 SOD1 1.06 0.76 1.06 0.106 0.461
核因子红细胞2相关因子2 Nrf2 0.99 0.88 0.98 0.043 0.545
NAD(P)H:醌氧化还原酶1 NQO1 1.00a 0.12b 0.27b 0.125 <0.001
血红素加氧酶1 HO-1 1.01a 0.21b 0.29b 0.118 <0.001
空肠Jejunum
过氧化氢酶CAT 0.97 0.86 1.08 0.100 0.705
谷胱甘肽过氧化物酶1 GPx1 0.98b 0.88b 1.48a 0.093 0.005
超氧化物歧化酶1 SOD1 1.07 0.97 1.24 0.102 0.627
核因子红细胞2相关因子2 Nrf2 1.04 0.77 0.93 0.100 0.617
NAD(P)H:醌氧化还原酶1 NQO1 0.98a 0.27b 0.47b 0.117 0.018
血红素加氧酶1 HO-1 0.95 0.93 1.33 0.112 0.307
回肠Ileum
过氧化氢酶CAT 1.00 0.93 1.19 0.109 0.663
谷胱甘肽过氧化物酶1 GPx1 1.00 0.93 1.49 0.124 0.119
超氧化物歧化酶1 SOD1 1.07a 0.51b 0.89a 0.092 0.019
核因子红细胞2相关因子2 Nrf2 1.04 0.91 0.96 0.070 0.771
NAD(P)H:醌氧化还原酶1 NQO1 0.98 0.65 1.53 0.173 0.088
血红素加氧酶1 HO-1 0.97 0.91 1.14 0.168 0.872

3 讨论

3.1 CKT对高精料育肥羔羊生长性能及营养物质表观消化率的影响

单宁进入动物消化道后,可与胃肠道黏膜表面的蛋白质或某些消化酶相互作用,形成难溶的单宁-蛋白质复合物,影响动物对营养物质的吸收和生长性能。然而近年来研究表明,饲粮中添加适量的单宁对动物生长性能不仅没有负面影响,还有积极的促进作用。Patra等[15]报道,草本植物中的单宁类物质可通过与蛋白质和脂质结合,有效抑制反刍动物消化道内细菌的增殖,显著改变其微生物群落组成。这种抑制作用能降低有害菌群对饲粮的降解率,提升动物对营养物质的吸收利用率,促进反刍动物的生长发育。张一平等[16]研究发现,在饲粮中添加20 g/(头·d)单宁提取物(栗木单宁+白坚木单宁)显著提高了西门塔尔育肥牛ADG,显著降低了F/G。然而本研究结果表明,在高精料饲粮中添加2 g/kg CKT并未对羔羊生长性能产生显著影响。由此可知,单宁对动物生长性能的影响受单宁来源、添加剂量以及试验动物种类等多种因素的影响。
营养物质表观消化率能直观反映动物机体对饲粮营养物质的消化吸收水平。高精料饲粮淀粉含量高,淀粉是育肥动物饲粮的主要成分和能量来源,未在瘤胃中消化的淀粉会进入小肠进行下一步消化。王璐[17]研究发现,羔羊采食精粗比为7∶3的高精料饲粮后,在短时间内(第3周)出现不良反应,导致营养物质表观消化率和ADG处于最低水平,但一段时间后,羔羊机体产生适应性反应,营养物质表观消化率和ADG可达到较高水平。Valdés等[18]研究发现,随着饲粮精粗比由2∶8提高至8∶2,绵羊DM和OM表观消化率显著升高。本课题组前期研究发现,采食精粗比为7∶3的高精料饲粮后,羔羊DM、CP、NDF和EE表观消化率显著升高[13]。本研究结果与上述结果相似,与CON组相比,HC组羔羊CP和EE表观消化率显著升高,可能原因是精料采食过多使非结构性碳水化合物比例升高,增加了饲粮在瘤胃及肠道中的停留时间,降低了饲粮流通速率,进而提高了营养物质表观消化率。
单宁来源多样且结构复杂,其作用效果可能存在差异。杨凯[19]研究表明,饲粮中添加26 g/kg的单宁酸显著降低了肉牛OM、DM和CP表观消化率。陈旭辉等[20]研究发现,饲粮中添加10 g/kg坚木单宁,会显著降低绒山羊ADF表观消化率。然而,Aguerre等[21]研究发现,饲粮中添加0.45%的单宁提取物对奶牛OM、DM和CP表观消化率无显著影响。本试验中,高精料饲粮中添加2 g/kg CKT对羔羊营养物质表观消化率无显著影响,与Aguerre等[21]的研究结果相似。肠道pH呈弱碱性,而单宁-蛋白质复合物在该环境中可被部分解离,促使更多的营养物质在小肠中被消化吸收,这可能是添加CKT后营养物质表观消化率未呈现显著差异的原因[22]

3.2 CKT对高精料育肥羔羊小肠形态结构的影响

小肠是动物营养物质消化吸收的主要场所,也是机体重要的免疫器官[23-24]。小肠形态结构的发育在肠道的消化和吸收过程中起着关键作用,肠绒毛是发挥吸收功能的主要结构,其发育状况常用VH和CD来衡量。其中,CD会影响肠绒毛有丝分裂形成上皮细胞的速度,反映隐窝细胞的增殖情况与成熟度,V/C则是评估肠道发育和功能的重要指标[25-26]。Lai等[27]研究发现,奶牛采食精粗比为4∶6的高谷物饲粮后,其小肠上皮刷状缘光滑平坦,结构完整;而采食精粗比为6∶4的高谷物饲粮后,其小肠上皮刷状缘出现凹陷和不规则形态,回肠绒毛损伤数量增加。薛春旭[28]研究发现,高精料饲粮能够提高山羊十二指肠、空肠和回肠VH,推测原因是该类饲粮营养物质含量高,增强了肠道的消化吸收能力;但山羊十二指肠、空肠和回肠CD升高,空肠V/C降低,且光学显微镜下可见回肠绒毛松散、排列不齐,这表明高精料饲粮可能会对小肠黏膜造成损伤。本试验结果表明,与CON组相比,HC组羔羊回肠VH和V/C显著降低,且HE染色结果表明,HC组羔羊小肠绒毛断裂、排列散乱,说明高精料饲粮导致羔羊小肠形态结构受损。其潜在机制可能是高精料饲粮引发动物机体氧化应激,进而激活炎症信号通路,使促炎因子释放,最终破坏小肠的物理屏障[29]
近年来大量研究表明,在动物饲粮中添加适宜剂量的单宁能改善肠道形态[30-31]。Wang等[32]报道,饲粮中添加200 mg/kg鞣花酸能够显著降低肉鸡十二指肠CD,显著提高十二指肠V/C和空肠VH、V/C。Liu等[33]研究发现,饲粮中添加2 g/kg栗木单宁显著提高了肉鸡空肠VH。本试验结果与上述结果相似,与HC组相比,CKT组羔羊回肠VH显著升高;空肠、回肠CD显著降低;十二指肠、回肠V/C显著升高。HE染色结果显示,与HC组相比,CKT组小肠绒毛生长较为紧密排列较为整齐,结构更加清晰。这可能是由于单宁-蛋白质复合物在肠道解离后,为肠道提供了营养物质,提高了隐窝细胞的增殖速率,促进隐窝基部细胞向绒毛端迁移、分化为具有吸收功能的成熟绒毛细胞,进而使VH增高、CD降低,改善了小肠肠道形态发育,缓解了高精料饲粮对羔羊肠道形态的损伤。

3.3 CKT对高精料育肥羔羊小肠抗氧化功能的影响

机体在健康状态下,自由基的产生与清除处于动态平衡;但在疾病状态下,自由基会大量堆积,当机体的抗氧化系统无法清除过多的自由基时,会打破机体氧化还原稳态,导致氧化应激。SOD、GPx和CAT等抗氧化酶是抵御氧化损伤的第1道防线,是细胞清除自由基主要的内源酶[34-35]。其中,SOD有利于维持超氧阴离子水平[36];GPx在保护身体免受氧化损伤方面起重要作用[37];CAT对保护细胞免受过氧化氢(H2O2)毒性影响具有积极作用[38]。T-AOC是衡量体内多种物质综合抗氧化水平的指标[39]。MDA是脂质过氧化的最终产物,若机体内多种氧自由基未得到清除,则会导致MDA蓄积[40]。大多数多酚类物质可充当自由基清除剂、供氢化合物和金属离子螯合剂[41]。Mu等[42]研究表明,在羔羊饲粮中添加40 mg/kg葡萄籽原花青素能显著提高结肠组织中T-AOC和GPx活性,并显著降低MDA含量。王思甜等[43]研究表明,灌服190 mg/kg单宁酸可显著提高感染猪流行性腹泻病毒的仔猪十二指肠和空肠GPx活性、结肠T-SOD活性以及十二指肠和结肠T-AOC。本课题组前期研究表明,给小鼠灌胃100 mg/kg CKT后其血清及肝脏T-SOD、CAT活性及T-AOC显著升高,血清MDA含量降低[14]。本试验结果表明,与HC组相比,CKT组羔羊回肠MDA含量显著降低。
Nrf2是抗氧化系统的主要调节因子,并且对氧化还原电位极为敏感[44]。在应激条件下,Nrf2会从Kelch样环氧氯丙烷相关蛋白1(Keap1)-Nrf2复合物中释放并迁移到细胞核内,与抗氧化反应元件(ARE)结合,进而激活抗氧化酶基因CATGPx1、SOD1、HO-1及NQO1的表达[45]。研究表明,植物多酚类物质主要通过激活Nrf2/ARE信号通路,调节机体内抗氧化酶基因的表达及提高抗氧化酶活性[46]。本课题组前期研究表明,在精粗比为7∶3的高精料饲粮中添加2 g/kg CKT显著上调了羔羊外周血淋巴细胞CATGPx1、SOD1、SOD2、Nrf2的mRNA相对表达量[13]。本试验结果表明,与CON组相比,HC组羔羊十二指肠NQO1和HO-1、空肠NQO1、回肠SOD1的mRNA相对表达量显著降低;而在高饲粮中添加2 g/kg CKT显著提高了羔羊十二指肠CAT、空肠GPx1、回肠SOD1的mRNA相对表达量。Huang等[47]研究表明,在仔猪饲粮中补充800 mg/kg苹果多酚可上调空肠黏膜SOD1及回肠黏膜Nrf2的mRNA相对表达量,下调空肠黏膜和回肠黏膜Keap1的mRNA相对表达量。牟春堂等[29]研究表明,饲粮中添加20、40 mg/kg BW的葡萄籽原花青素显著上调了羔羊结肠组织中Nrf2、HO-1、GPx4基因和蛋白的表达量。综合以上结果,CKT有可能通过调节Keap1/Nrf2信号通路增强动物肠道抗氧化能力,从而有效缓解肠道氧化损伤。

4 结论

高精料饲粮中添加2 g/kg CKT,可在不影响育肥羔羊生长性能的前提下,通过改善小肠形态结构、调节小肠MDA含量及抗氧化相关基因的表达提高羔羊抗氧化功能,缓解高精料饲粮引发的小肠氧化损伤,进而促进机体健康。
[1]
OHTAKI T, OGATA K N, KAJIKAWA H, et al. Effect of high-concentrate corn grain diet-induced elevated ruminal lipopolysaccharide levels on dairy cow liver function[J]. Journal of Veterinary Medical Science, 2020, 82(7):971-977.

DOI PMID

[2]
CHEN M R, XIE W, ZHOU S D, et al. A high-concentrate diet induces colonic inflammation and barrier damage in Hu sheep[J]. Journal of Dairy Science, 2023, 106(12):9644-9662.

[3]
MA N, ABAKER J A, WEI G, et al. A high-concentrate diet induces an inflammatory response and oxidative stress and depresses milk fat synthesis in the mammary gland of dairy cows[J]. Journal of Dairy Science, 2022, 105(6):5493-5505.

[4]
YANG W G, GUO G Z, CHEN J Y, et al. Effects of dietary fucoidan supplementation on serum biochemical parameters,small intestinal barrier function,and cecal microbiota of weaned goat kids[J]. Animals, 2022, 12(12):1591.

[5]
PLAIZIER J C, KHAFIPOUR E, LI S, et al. Subacute ruminal acidosis (SARA),endotoxins and health consequences[J]. Animal Feed Science and Technology, 2012, 172(1/2):9-21.

[6]
RAJKOVIĆ E, SCHWARZ C, KAPSAMER S B, et al. Evaluation of a dietary grape extract on oxidative status,intestinal morphology,plasma acute-phase proteins and inflammation parameters of weaning piglets at various points of time[J]. Antioxidants, 2022, 11(8):1428.

[7]
李杰, 刘巧玲, 孙红先, 等. 植物单宁营养生理功能及其在反刍动物生产中的应用研究进展[J]. 畜牧兽医杂志, 2021, 40(6):79-82.

LI J, LIU Q L, SUN H X, et al. Research progress on nutritional and physiological functions of plant tannins and their application in ruminant production[J]. Journal of Animal Science and Veterinary Medicine, 2021, 40(6):79-82. (in Chinese)

[8]
KHANBABAEE K, VAN REE T. Tannins:classification and definition[J]. Natural Product Reports, 2001, 18(6):641-649.

[9]
TRUONG V L, JEONG W S. Antioxidant and anti-inflammatory roles of tea polyphenols in inflammatory bowel diseases[J]. Food Science and Human Wellness, 2022, 11(3):502-511.

[10]
PELEGRIN-VALLS J, ÁLVAREZ-RODRÍGUEZ J, MARTÍN-ALONSO M J. Effect of maternal dietary condensed tannins from sainfoin (Onobrychis viciifolia) on gut health and antioxidant-immune crosstalk in suckling lambs[J]. Agriculture, 2022, 12(10):1694.

[11]
GUO Z Y, CHEN X L, HUANG Z Q, et al. Apple polyphenols improve intestinal barrier function by enhancing antioxidant capacity and suppressing inflammation in weaning piglets[J]. Animal Science Journal, 2022, 93(1):e13747.

[12]
YU J, SONG Y Y, YU B, et al. Tannic acid prevents post-weaning diarrhea by improving intestinal barrier integrity and function in weaned piglets[J]. Journal of Animal Science and Biotechnology, 2020,11:87.

[13]
陈治宇. 柠条单宁对高精料育肥羔羊生长性能、免疫和抗氧化功能的影响[D]. 硕士学位论文. 呼和浩特: 内蒙古农业大学, 2024.

CHEN Z Y. Effects of Caragana korshinskii tannin on growth performance,immune and antioxidant function of high concentrate fattening lambs[D]. Master’s Thesis. Hohhot: Inner Mongolia Agricultural University, 2024. (in Chinese)

[14]
曲魏. 柠条单宁的提取及其对小鼠生长性能,免疫和抗氧化功能的影响[D]. 硕士学位论文. 呼和浩特: 内蒙古农业大学, 2023.

QU W. Extraction of Caragana korshinskii tannin and its effects on growth performance,immunity and antioxidant function in mice[D]. Master’s Thesis. Hohhot: Inner Mongolia Agricultural University, 2023. (in Chinese)

[15]
PATRA A K, SAXENA J. The effect and mode of action of saponins on the microbial populations and fermentation in the rumen and ruminant production[J]. Nutrition Research Reviews, 2009, 22(2):204-219.

DOI PMID

[16]
张一平, 田雨晴, 李秋凤, 等. 单宁提取物对西门塔尔育肥牛生长性能、营养物质表观消化率、血清生化和抗氧化指标的影响[J]. 动物营养学报, 2024, 36(3):1713-1723.

DOI

ZHANG Y P, TIAN Y Q, LI Q F, et al. Effects of tannin extract on growth performance,nutrient apparent digestibility,serum biochemical and antioxidant indices of Simmental fattening cattle[J]. Chinese Journal of Animal Nutrition, 2024, 36(3):1713-1723. (in Chinese)

[17]
王璐. 比较研究粉碎和整粒玉米高精料日粮对育肥羔羊生长性能、瘤胃微生物区系和上皮形态功能的影响[D]. 硕士学位论文. 南京: 南京农业大学, 2022.

WANG L. Comparative study of the effects of ground and whole corn high-grain diets on growth performance,ruminal bacterial community,and ruminal epithelial morphology and function in fattening lambs[D]. Master’s Thesis. Nanjing: Nanjing Agricultural University, 2022. (in Chinese)

[18]
VALDÉS C, CARRO M D, RANILLA M J. et al. Effect of forage to concentrate ratio in complete diets offered to sheep on voluntary food intake and some digestive parameters[J]. Animal Science, 2000, 70(1):119-126.

[19]
杨凯. 单宁酸对肉牛瘤胃发酵、微生物区系、甲烷排放及氮排泄的调控规律[D]. 博士学位论文. 北京: 中国农业大学, 2017.

YANG K. Manipulation of tannic acid on rumen fermentation,microbial flora,methane emission and nitrogen excretion in beef cattle[D]. Ph.D.Thesis. Beijing: China Agricultural University, 2017. (in Chinese)

[20]
陈旭辉, 张子怡, 王春艳, 等. 饲粮中添加坚木单宁对辽宁绒山羊生长性能、营养物质消化代谢和抗氧化能力的影响[J]. 动物营养学报, 2024, 36(10):6468-6478.

DOI

CHEN X H, ZHANG Z Y, WANG C Y, et al. Effects of dietary quebracho tannin supplementation on growth performance,nutrient digestion and metabolism,and antioxidant capacity of Liaoning cashmere goats[J]. Chinese Journal of Animal Nutrition, 2024, 36(10):6468-6478. (in Chinese)

[21]
AGUERRE M J, CAPOZZOLO M C, LENCIONI P, et al. Effect of quebracho-chestnut tannin extracts at 2 dietary crude protein levels on performance,rumen fermentation,and nitrogen partitioning in dairy cows[J]. Journal of Dairy Science, 2016, 99(6):4476-4486.

[22]
NAUMANN H D, TEDESCHI L O, ZELLER W E, et al. The role of condensed tannins in ruminant animal production: advances,limitations and future directions[J]. Revista Brasileira de Zootecnia, 2017, 46(12):929-949.

[23]
HELANDER H F, FÄNDRIKS L. Surface area of the digestive tract-revisited[J]. Scandinavian Journal of Gastroenterology, 2014, 49(6),681-689.

[24]
CELI P, COWIESON A J, FRU-NJI F, et al. Gastrointestinal functionality in animal nutrition and health:new opportunities for sustainable animal production[J]. Animal Feed Science and Technology, 2017,234:88-100.

[25]
LIU Y, LIN Q, HUANG X, et al. Effects of dietary ferulic acid on the intestinal microbiota and the associated changes on the growth performance,serum cytokine profile,and intestinal morphology in ducks[J]. Frontiers in Microbiology, 2021,12:698213.

[26]
HU Y N, WANG Y W, LI A K, et al. Effects of fermented rapeseed meal on antioxidant functions,serum biochemical parameters and intestinal morphology in broilers[J]. Food and Agricultural Immunology, 2016, 27(2):182-193.

[27]
LAI Z, LIN L, ZHANG J, et al. Effects of high-grain diet feeding on mucosa-associated bacterial community and gene expression of tight junction proteins and inflammatory cytokines in the small intestine of dairy cattle[J]. Journal of Dairy Science, 2022, 105(8):6601-6615.

DOI PMID

[28]
薛春旭. 高精料日粮对山羊小肠微生物发酵、微生物区系及上皮形态结构的影响[D]. 硕士学位论文. 南京: 南京农业大学, 2017.

XUE C X. The impact of high concentrate diet on small intestinal fermentation,microbial community and epithelial morphology of goats[D]. Master’s Thesis. Nanjing: Nanjing Agricultural University, 2017. (in Chinese)

[29]
牟春堂, 魏焕, 谢蕴哲, 等. 葡萄籽原花青素对饲喂高精料绵羊结肠上皮屏障的影响及作用机制研究[J]. 中国畜牧兽医, 2024, 51(10):4270-4281.

DOI

MU C T, WEI H, XIE Y Z, et al. Effect of grape seed proanthocyanidins on colon epithelial barrier of sheep fed a high-concentrate diet and its mechanism[J]. China Animal Husbandry & Veterinary Medicine, 2024, 51(10):4270-4281. (in Chinese)

[30]
ZHAO M D, DI L F, TANG Z Y, et al. Effect of tannins and cellulase on growth performance,nutrients digestibility,blood profiles,intestinal morphology and carcass characteristics in Hu sheep[J]. Asian-Australasian Journal of Animal Sciences, 2019, 32(10):1540-1547.

[31]
WU Q J, WANG Y Q, QI Y X. The protective effect of procyanidin against LPS-induced acute gut injury by the regulations of oxidative state[J]. SpringerPlus, 2016, 5(1):1645.

PMID

[32]
WANG F, CHEN J S, YIN Y X, et al. The effects of dietary ellagic acid supplementation on growth performance,immune response,antioxidant activity,digestive enzyme activities,and intestinal functions in yellow-feathered broilers[J]. Journal of Animal Science, 2022, 100(12):skac301.

[33]
LIU H W, LI K, ZHAO J S, et al. Effects of chestnut tannins on intestinal morphology,barrier function,pro-inflammatory cytokine expression,microflora and antioxidant capacity in heat-stressed broilers[J]. Journal of Animal Physiology and Animal Nutrition, 2018, 102(3):717-726.

[34]
ZHAO J X, LI Q, ZHANG R X, et al. Effect of dietary grape pomace on growth performance,meat quality and antioxidant activity in ram lambs[J]. Animal Feed Science and Technology, 2018,236:76-85.

[35]
ZHAO J X, LI K, SU R, et al. Effect of dietary tartary buckwheat extract supplementation on growth performance,meat quality and antioxidant activity in ewe lambs[J]. Meat Science, 2017,134:79-85.

[36]
WANG Y, BRANICKY R, NOË A, et al. Superoxide dismutases:dual roles in controlling ROS damage and regulating ROS signaling[J]. The Journal of Cell Biology, 2018, 217(6):1915-1928.

[37]
PEI J, PAN X Y, WEI G H, et al. Research progress of glutathione peroxidase family (GPX) in redoxidation[J]. Frontiers in Pharmacology, 2023,14:1147414.

[38]
NANDI A, YAN L J, JANA C K, et al. Role of catalase in oxidative stress- and age-associated degenerative diseases[J]. Oxidative Medicine and Cellular Longevity, 2019,2019:9613090.

[39]
SAHIN K, ORHAN C, TUZCU M, et al. Lycopene activates antioxidant enzymes and nuclear transcription factor systems in heat-stressed broilers[J]. Poultry Science, 2016, 95(5):1088-1095.

DOI PMID

[40]
WANG F, YIN Y X, YANG M, et al. Effects of combined supplementation of Macleaya cordata extract and benzoic acid on the growth performance,immune responses,antioxidant capacity,intestinal morphology,and microbial composition in weaned piglets[J]. Frontiers in Veterinary Science, 2021,8:708597.

[41]
KIM D O, LEE K W, LEE H J, et al. Vitamin C equivalent antioxidant capacity (VCEAC) of phenolic phytochemicals[J]. Journal of Agricultural and Food Chemistry, 2002, 50(13):3713-3717.

[42]
MU C T, HAO X Y, ZHANG X Z, et al. Effects of high-concentrate diet supplemented with grape seed procyanidins on the colonic fermentation,colonic morphology,and inflammatory response in lambs[J]. Animal Feed Science and Technology, 2021,281:115118.

[43]
王思甜, 徐朋涛, 郑丽云, 等. 单宁酸对感染猪流行性腹泻病毒仔猪生长性能、肠道屏障功能和抗氧化能力的影响[J]. 动物营养学报, 2023, 35(7):4276-4286.

DOI

WANG S T, XU P T, ZHENG L Y, et al. Effects of tannin acid on growth performance,intestinal barrier function and antioxidant capacity of piglets infected with porcine epidemic diarrhea virus[J]. Chinese Journal of Animal Nutrition, 2023, 35(7):4276-4286. (in Chinese)

[44]
CHEN Q M. Nrf2 for protection against oxidant generation and mitochondrial damage in cardiac injury[J]. Free Radical Biology & Medicine, 2022,179:133-143.

[45]
DING X Q, JIAN T Y, WU Y X, et al. Ellagic acid ameliorates oxidative stress and insulin resistance in high glucose-treated HepG2 cells via miR-223/Keap1-Nrf2 pathway[J]. Biomedicine & Pharmacotherapy, 2019,110:85-94.

[46]
赵欣, 骞宇. 苦丁茶粗多酚对DSS诱导C57BL/6J小鼠溃疡性结肠炎的预防作用[J]. 食品工业科技, 2017, 38(9):357-362.

ZHAO X, QIAN Y. Preventive effects of Kuding tea crude polyphenols in DSS-induced C57BL/6J mice ulcerative colitis[J]. Science and Technology of Food Industry, 2017, 38(9):357-362. (in Chinese)

[47]
HUANG T T, CHE Q J, CHEN X L, et al. Apple polyphenols improve intestinal antioxidant capacity and barrier function by activating the Nrf2/Keap1 signaling pathway in a pig model[J]. Journal of Agricultural and Food Chemistry, 2022, 70(24):7576-7585.

DOI PMID

Outlines

/