RESEARCH PAPER

Effects of Diets with Different Roughage Sources on Intestinal Immune Function of Yak Calves during Lactation Based on Transcriptomics Analysis

  • BO Fuquan ,
  • AN Lele ,
  • ZHOU Ya’nan ,
  • YANG Deyu ,
  • ZHANG Xiaowei ,
  • LIU Shujie ,
  • CUI Zhanhong , **
Expand
  • Key Laboratory of Plateau Grazing Animal Nutrition and Feed Science of Qinghai Province, Yak Engineering Technology Research Center of Qinghai Province, Ministry of Agriculture and Rural Affairs Key Laboratory of Animal Nutrition and Forage-Feed of Grazing Yak and Tibetan Sheep in Qinghai-Tibetan Plateau, Qinghai Academy of Animal Husbandry and Veterinary Sciences in Qinghai University, Xining 810016, China
**professor, E-mail:

*Contributed equally

Received date: 2024-11-30

  Online published: 2025-08-14

Abstract

This experiment aimed to explore the effects of diets with different roughage sources (oat hay, alfalfa hay and their mixed hay) on intestinal immune function of yak calves during lactation based on transcriptomics analysis. Twenty-one healthy male yak calves at 45 days of age with body weight of (36.47±0.99) kg were randomly divided into 3 groups (7 calves in each group) using a single-factor experimental design: the alfalfa hay group (AH group), the oat hay group (OH group) and the mixed hay group (AO group, alfalfa hay∶oat hay= 1∶1). The calves in each group were fed the same amount of milk replacer, concentrate and hay, with a concentrate-to-forage ratio of 3∶7. When the solid dry matter intake reached 1 kg/d, five calves from each group were slaughtered, and the jejunum and colon tissues were collected for transcriptomic sequencing and analysis. The pre-feeding period was 21 days, and the formal experimental period was 120 days. The results showed as follows: 1) the transcriptome analysis of jejunum showed that there were 100 3 differentially expressed genes (DEGs) between the AO and AH groups, 1 553 DEGs between the OH and AH groups, and 919 DEGs between the AO and OH groups. The GO enrichment analysis indicated that 680 GO terms were annotated by the DEGs between the AH and OH groups, 646 GO terms by the DEGs between the AH and AO groups, and 606 GO terms by the DEGs between the AO and OH groups. The KEGG enrichment analysis showed that the AO group mainly enhanced the immune function of jejunum by activating the complement and coagulation cascades and antigen processing and presentation. 2) The transcriptome analysis of colon showed that there were 3 362 DEGs between the AO and AH groups, 1 299 DEGs between the OH and AH groups, and 1 297 DEGs between the AO and OH groups. The GO enrichment analysis indicated that 665 GO terms were annotated by the DEGs between the AH and OH groups, 869 GO terms by the DEGs between the AH and AO groups, and 695 GO terms by the DEGs between the AO and OH groups. The KEGG enrichment analysis showed that the AO group mainly enhanced the immune function of colon by activating the chemokine signaling pathway and tight junctions. In conclusion, feeding the mixed hay increase promote the expression of immune related genes in jejunum and colon, regulate the intestinal immune response ability and health level, which is conducive to the healthy and high-quality cultivation of yak calves during the lactation period.

Cite this article

BO Fuquan , AN Lele , ZHOU Ya’nan , YANG Deyu , ZHANG Xiaowei , LIU Shujie , CUI Zhanhong . Effects of Diets with Different Roughage Sources on Intestinal Immune Function of Yak Calves during Lactation Based on Transcriptomics Analysis[J]. Chinese Journal of Animal Nutrition, 2025 , 37(8) : 5501 -5513 . DOI: 10.12418/CJAN2025.446

哺乳期是动物生长发育的关键阶段,哺乳期营养状况影响幼畜生长、健康及未来生产性能。牦牛是青藏高原优势畜种,对当地牧民经济收入和生活质量十分重要,其犊牛高质量培育是产业持续发展的关键基础。青藏高原恶劣的自然条件使牦牛犊牛营养需求敏感,肠道作为营养吸收主器官,其健康状况与功能对牦牛犊牛生长发育起决定性作用[1]。因此,深入探讨不同粗饲料来源对牦牛犊牛肠道健康及功能的影响,对于优化饲养管理策略和提高生产效率具有重要意义。
苜蓿干草富含蛋白质、维生素和矿物质,且钙含量高,有利于犊牛骨骼健康发展;其粗纤维有助于维持正常消化道运动,促进肠道健康。燕麦干草能量密度高、适口性好,可提供必需能量满足牦牛犊牛快速生长需求,适量纤维有助于消化系统发育健康[2]。等比例混合苜蓿干草与燕麦干草,可互补营养成分,确保饲料营养的全面性[3]。通过合理调整饲料配方可优化犊牛饲粮结构,可提高饲草料的消化利用率,以满足犊牛能量、蛋白质的需求,促进肠道功能发育,进而提高犊牛早期培育质量。为满足牦牛犊牛的营养需求,保证其健康高质量的生长发育,本研究选用苜蓿干草、燕麦干草及二者1∶1等比例混合干草作为试验饲粮的粗饲料来源,采用转录组学测序技术探究不同粗饲料来源饲粮对哺乳期牦牛犊牛肠道组织基因表达的影响,阐释其对肠道组织发育及相关功能基因表达的调控作用,旨在揭示饲粮营养水平与牦牛犊牛肠道健康的关系,为优化牦牛幼畜饲养管理、提高高原畜牧业生产效益提供重要参考。

1 材料与方法

1.1 试验设计

动物试验已由青海大学畜牧兽医科学院实验动物管理委员会批准,审批号:2022-QHMKY-015。
试验选择45日龄、体重(36.47±0.99) kg的健康牦牛犊牛(公)21头,随机分为3组,每组7头牛。各组分别饲喂苜蓿干草(AH组)、燕麦干草(OH组)和苜蓿干草∶燕麦干草=1∶1的混合干草(AO组),以及相同的代乳粉和开食料。预试期21 d,正试期120 d。代乳粉和开食料购自北京精准动物营养研究中心,燕麦干草产自青海,苜蓿干草产自甘肃张掖。代乳粉、开食料、苜蓿干草和燕麦干草营养水平见周亚楠等[4]

1.2 饲养管理

本试验在青海省海晏县高原现代生态畜牧业科技试验示范园开展,牦牛犊牛单栏饲养,栏舍光照充足,犊牛可自由活动与饮水。预试期完成饲粮和饲养管理过渡,结束后各组牦牛犊牛已适应代乳粉、开食料和干草。正式试验期间,每日08:30、16:30各饲喂1次,代乳粉冲泡及饲粮饲喂方法参考周亚楠等[4],开食料和干草分开饲喂,先精后粗,精粗比为3∶7。

1.3 样品采集与处理

饲养试验结束后,每组屠宰5头牦牛犊牛,结扎分离各肠断,采集空肠和结肠中端,用生理盐水冲洗后,放入含4%多聚甲醛溶液的速冻管中固定,每日更换溶液至澄清。最后取每段肠道中部组织黏膜,置于5 mL无菌冻存管,立即投入到液氮中,再转存到-80 ℃冰箱待测。

1.4 转录组文库构建及测序

将15头牦牛犊牛空肠和结肠组织样品送至北京诺禾致源科技股份有限公司开展转录组测序:先用TRIzol(日本TaKaRa公司)试剂法从空肠、结肠黏膜样本提取总RNA,并以Agilent 2100 Bioanalyzer评估其完整性与总量;文库构建时富集mRNA、随机打断,合成cDNA双链并连测序接头,选合适片段PCR扩增纯化,再定量质检查库以符测序要求。数据质控中去除含接头序列、不确定碱基信息(N)或低质量reads,统计clean data的Q20、Q30及GC含量。随后用HISAT2软件将reads与参考基因组比对,再用String Tie软件组装新转录本,feature Counts计算FPKM值定量基因表达,依log2[差异倍数(FC)]>1且校正P值(P-adjust)<0.05筛选差异表达基因(differentially expressed genes,DEGs),最后以P-adjust<0.05为标准通过GO和KEGG途径分析差异表达基因功能富集情况。

2 结果与分析

2.1 牦牛犊牛空肠和结肠差异表达基因筛选

表1所示,空肠差异表达基因:AH组vs AO组共1 003个,AH组vs OH组共1 553个,AO组vs OH组共919个;结肠差异表达基因:AH组vs AO组共3 362个,AH组vs OH组共1 299个,AO组vs OH组共1 297个。
表1 差异比较组别差异表达基因条目统计表

Table 1 Statistical table of differentially expressed gene counts in differential comparison groups

项目
Items
组别比较
Group comparison
总数
Total
上调
Up-regulated
下调
Down-regulated

空肠
Jejunum
AH组vs AO组AH group vs AO group 1 003 509 494
AH组vs OH组AH group vs OH group 1 553 838 715
AO组vs OH组AO group vs OH group 919 438 481

结肠
Colon
AH组vs AO组AH group vs AO group 3 362 1 784 1 578
AH组vs OH组AH group vs OH group 1 299 804 495
AO组vs OH组AO group vs OH group 1 297 560 737

2.2 牦牛犊牛空肠差异表达基因的GO和KEGG富集分析

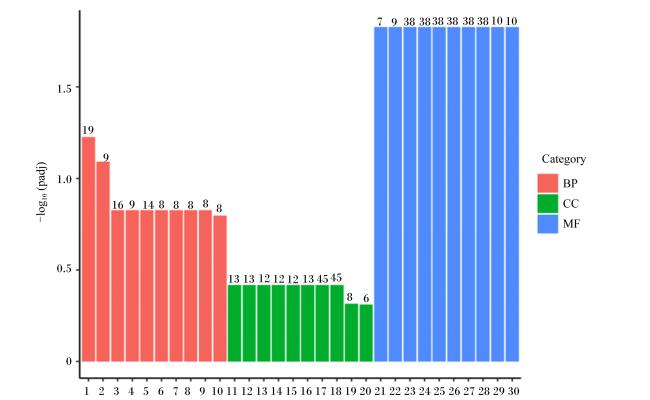
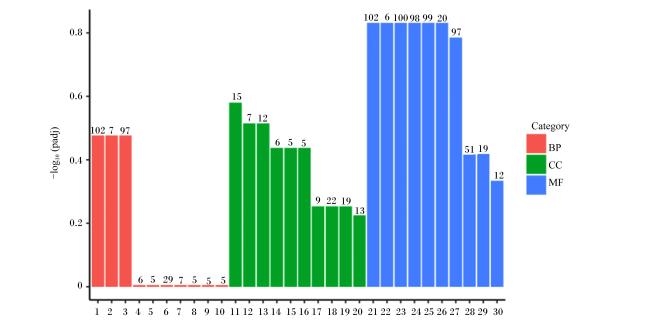
GO功能注释分为三大类:细胞组分(cellular component,CC)、分子功能(molecular function,MF)和生物学过程(biological process,BP)。对牦牛犊牛空肠差异表达基因进行GO富集分析,选取最显著的30个功能绘制柱状图,差异表达基因在BP、CC和MF三大类中均有富集。如图1所示,AH组vs OH组在BP、MF及CC三大类中,差异表达基因所富集的GO条目分别为341、92和247条。在BP中,差异表达基因主要富集在免疫系统进程、蛋白质折叠和免疫反应等;在CC中,差异表达基因主要富集在核小体、蛋白质-DNA复合体、DNA包装复合体等;在MF中,差异表达基因主要富集在未折叠蛋白结合、三磷酸鸟苷结合和核糖核苷结合等。
图1 牦牛犊牛空肠差异表达基因GO功能富集分析(AH组vs OH组)

padj:校正PP-adjust;Category:类别;BP:生物过程 biological process;CC:细胞组分 cellular component;MF:分子功能 molecular function;图2图6同 the same as Fig.2 to Fig.6

1:免疫系统过程 immune system process;2:蛋白质折叠 protein folding;3:免疫反应 immune response;4:DNA构象变化 DNA conformation change;5:细胞蛋白质复合体组装 cellular protein-containing complex assembly;6:核小体组装 nucleosome assembly;7:染色质组装 chromatin assembly;8:DNA包装 DNA packaging;9:核小体组织 nucleosome organization;10:染色质组装或解组装 chromatin assembly or disassembly;11:细胞骨架部分 cytoskeletal part;12:染色质 chromatin;13:核小体 nucleosome;14:蛋白质-DNA复合体 protein-DNA complex;15:DNA包装复合体 DNA packaging complex;16:细胞骨架 cytoskeleton;17:非膜包被细胞器 non-membrane-bounded organelle;18:胞内非膜包被细胞器 intracellular non-membrane-bounded organelle;19:肌动蛋白细胞骨架 actin cytoskeleton;20:肌球蛋白复合体 myosin complex;21:细胞外基质结构成分 extracellular matrix structural constituent;22:未折叠蛋白结合 unfolded protein binding;23:纯核苷酸结合 purine nucleoside binding;24:三磷酸鸟苷结合 GTP binding;25:核糖核苷酸结合 ribonucleoside binding;26:纯核糖核苷酸结合 purine ribonucleoside binding;27:核苷酸结合 nucleoside binding;28:鸟苷核糖核苷酸结合 guanyl ribonucleoside binding;29:内肽酶抑制剂活性 endopeptidase inhibitor activity;30:内肽酶调节器活性endopeptidase regulator activity。

Fig.1 GO functional enrichment analysis of differently expressed genes in jejunum of yak calves (AH group vs OH group)

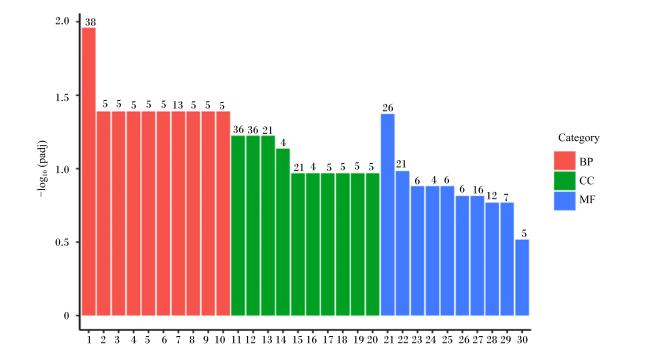
图2所示,AH组vs AO组在BP、MF及CC三大类中,差异表达基因所富集的GO条目分别为329、81和236条。在BP中,差异表达基因主要富集在有机氮化合物生物合成过程、核苷三磷酸生物合成过程和纯核苷三磷酸生物合成过程等;在CC中,差异表达基因主要富集在非膜包被细胞器、胞内非膜包被细胞器、核糖体、核糖核蛋白复合物和微管相关复合体等;在MF中,差异表达基因主要富集在结构分子活性、核糖体的结构成分和脂肪酶活性等。
图2 牦牛犊牛空肠差异表达基因GO功能富集分析(AH组vs AO组)

1:有机氮化合物生物合成过程 organonitrogen compound biosynthetic process;2:ATP生物合成过程 ATP biosynthetic process;3:核苷三磷酸生物合成过程 nucleoside triphosphate biosynthetic process;4:纯核苷三磷酸生物合成过程 purine nucleoside triphosphate biosynthetic process;5:核糖核苷三磷酸生物合成过程 ribonucleoside triphosphate biosynthetic process;6:嘌呤核糖核苷三磷酸生物合成过程 purine ribonucleoside triphosphate biosynthetic process;7:碳水化合物衍生物生物合成过程 carbohydrate derivative biosynthetic process;8:核苷一磷酸生物合成过程 nucleoside monophosphate biosynthetic process;9:嘌呤核苷一磷酸生物合成过程 purine nucleoside monophosphate biosynthetic process;10:核糖核苷一磷酸生物合成过程 ribonucleoside monophosphate biosynthetic process;11:非膜包被细胞器 non-membrane-bounded organelle;12:胞内非膜包被细胞器 intracellular non-membrane-bounded organelle;13:核糖体 ribosome;14:动力蛋白复合体 dynein complex;15:核糖核蛋白复合体 ribonucleoprotein complex;16:微管相关复合体 microtubule associated complex;17:内质网膜 endoplasmic reticulum membrane;18:内质网亚区室 endoplasmic reticulum subcompartment;19:核外膜-内质网膜 nuclear outer membrane-endoplasmic reticulum membrane;20:内质网部分 endoplasmic reticulum part;21:结构分子活性 structural molecule activity;22:核糖体的结构成分 structural constituent of ribosome;23:转移酶活性,转移戊糖基团 transferase activity, transferring pentosyl groups;24:磷脂酶A2活性 phospholipase A2 activity;25:羧酸酯水解酶活性 carboxylic ester hydrolase activity;26:脂肪酶活性 lipase activity;27:转移酶活性,转移糖基团 transferase activity, transferring glycosyl groups;28:辅酶结合 coenzyme binding;29:微管马达活性 microtubule motor activity;30:磷脂酶活性 phospholipase activity。

Fig.2 GO functional enrichment analysis of differently expressed genes in jejunum of yak calves (AH group vs AO group)

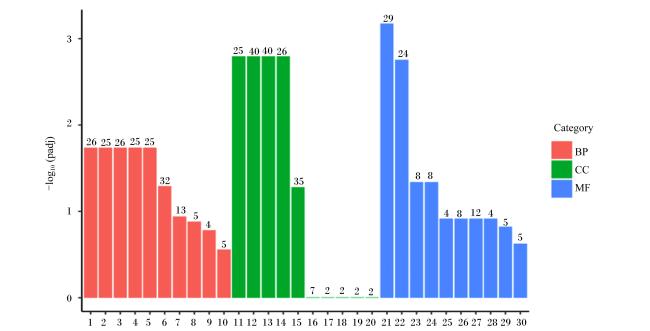
图3所示,AO组vs OH组在BP、MF及CC三大类中,差异表达基因所富集的GO的条目分别为323、75和208条。在BP中,差异表达基因主要富集在肽代谢过程、翻译和肽生物合成过程等;在CC中,差异表达基因主要富集在核糖体和核糖核蛋白复合物等;在MF中,差异表达基因主要富集在结构分子活性、核糖体的结构成分和肽酶抑制剂活性等。
图3 牦牛犊牛空肠差异表达基因GO功能富集分析(AO组vs OH组)

1:肽代谢过程 peptide metabolic process;2:翻译 translation;3:细胞酰胺代谢过程 cellular amide metabolic process;4:肽生物合成过程 peptide biosynthetic process;5:酰胺生物合成过程 amide biosynthetic process;6:有机氮化合物生物合成过程 organonitrogen compound biosynthetic process;7:碳水化合物代谢过程 carbohydrate metabolic process;8:含核碱基化合物的分解代谢过程 nucleobase-containing compound catabolic process;9:细胞氮化合物生物合成过程 cellular nitrogen compound biosynthetic process;10:细胞氮化合物分解代谢过程 cellular nitrogen compound catabolic process;11:核糖体 ribosome;12:非膜包被细胞器 non-membrane-bounded organelle;13:胞内非膜包被细胞器 intracellular non-membrane-bounded organelle;14:核糖核蛋白复合体 ribonucleoprotein complex;15:细胞质部分 cytoplasmic part;16:染色质 chromatin;17:外囊复合体 exocyst;18:细胞皮层 cell cortex;19:细胞皮层部分 cell cortex part;20:细胞质区域 cytoplasmic region;21:结构分子活性 structural molecule activity;22:核糖体的结构成分 structural constituent of ribosome;23:肽酶抑制剂活性 peptidase inhibitor activity;24:肽酶调节器活性 peptidase regulator activity;25:细胞外基质结构成分 extracellular matrix structural constituent;26:酶抑制剂活性 enzyme inhibitor activity;27:核苷三磷酸酶活性 ATPase activity;28:rRNA结合 rRNA binding;29:未折叠蛋白结合 unfolded protein binding;30:羧酸酯水解酶活性 carboxylic ester hydrolase activity。

Fig.3 GO functional enrichment analysis of differently expressed genes in jejunum of yak calves (AO group vs OH group)

对牦牛犊牛空肠差异表达基因进行KEGG富集分析。如表2所示,AH组vs OH组的差异表达基因主要富集在焦点黏连和细胞外基质受体相互作用等通路;AO组vs AH组的差异表达基因主要富集在补体和凝血级联通路;AO组vs OH组的差异表达基因主要富集在抗原处理与呈递、蛋白质消化与吸收补体和凝血级联反应等通路。
表2 空肠的差异表达基因及其KEGG富集通路

Table 2 Differentially expressed genes in jejunum and its KEGG-enriched pathways

KEGG通路
KEGG pathways
上调差异表达
基因数目
Number of
up-regulated DEGs
下调差异表达
基因数目
Number of
down-regulated
DEGs
主要上调差异
表达基因
Main up-regulated
DEGs
主要下调差异
表达基因
Main down-regulated
DEGs
AH组vs OH组AH group vs OH group
焦点黏连
Focal adhesion
27 5 PPP1R12A/
COL6A2/FN1
LAMC2/
PAK6/PXN
细胞外基质受体相互作用
ECM-receptor interaction
13 4 COL1A2/FN1/ITGA5 LAMC2
AO组vs AH组AO group vs AH group
补体和凝血级联
Complement and coagulation cascades
5 15 MASP1/C4/F7 C4BPB/CFI/C8B
AO组vs OH组AO group vs OH group
抗原处理与呈递
Antigen processing and presentation
5 13 CⅡTA/CD8B LGMN/HSPA5/CTSV
蛋白质消化与吸收
Protein digestion and absorption
3 8 SLC9A3/SLC3A1 COL23A1/COL5A3
补体和凝血级联反应
Complement and coagulation cascades
2 8 MASP1/FGG CD59/C8B

PPP1R12A:蛋白磷酸酶1调节亚基12A protein phosphatase 1 regulatory subunit 12A;COL6A2:胶原蛋白VI型α2链 collagen type Ⅵ alpha 2 chain;FN1:纤维连接蛋白1 fibronectin 1;LAMC2:层黏连蛋白γ2链 laminin subunit gamma 2;PAK6:p21激活激酶6 p21 activated kinase 6;PXN:斑点蛋白 paxillin;COL1A2:胶原蛋白Ⅰ型α2链 collagen type Ⅰ alpha 2 chain;ITGA5:整合素α5 integrin alpha 5;LAMC2:层黏连蛋白γ2链 laminin subunit gamma 2;MASP1:甘露糖结合凝集素丝氨酸蛋白酶1 mannan-binding lectin serine protease 1;C4:补体成分4 complement component 4;F7:凝血因子Ⅶ coagulation factor Ⅶ;C4BPB:补体成分4结合蛋白β链 complement component 4 binding protein beta;CFⅠ:补体因子Ⅰ complement factor Ⅰ;C8B:补体成分8 β链 complement component 8 beta;CⅡTA:主要组织相容性复合体Ⅱ类转录激活因子 MHC class Ⅱ transactivator;CD8B:CD8β分子 CD8 molecule beta chain;LGMN:腿氨酸蛋白酶 legumain;HSPA5:热休克蛋白A5 heat shock protein family A member 5;CTSV:组织蛋白酶V cathepsin V;SLC9A3:溶质载体家族9成员A3 solute carrier family 9 member A3;SLC3A1:溶质载体家族3成员A1 solute carrier family 3 member A1;COL23A1:ⅩⅩⅢ型胶原蛋白α1链 collagen type ⅩⅩⅢ alpha 1 chain;COL5A3:Ⅴ型胶原蛋白α3链 collagen type Ⅴ alpha 3 chain;FGG:纤维蛋白原 fibrinogen;CD59:CD59分子 CD59 molecule。

2.3 牦牛犊牛结肠差异表达基因的GO富集和KEGG富集分析

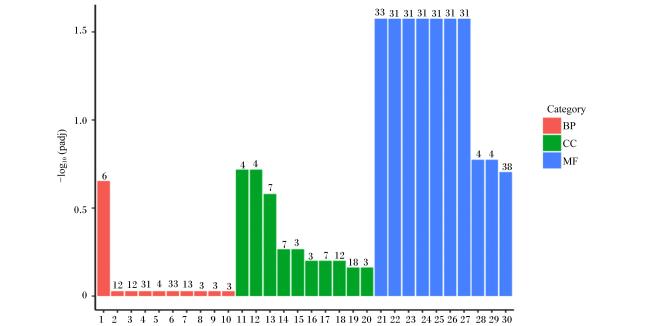
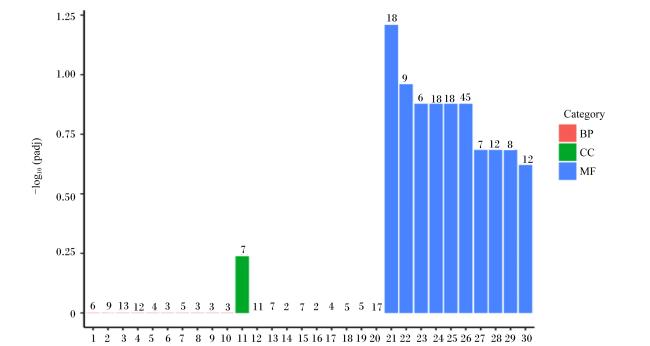
对牦牛犊牛结肠差异表达基因进行GO富集分析,选取最显著的30个功能绘制柱状图,差异表达基因在BP、CC和MF三大类中均有富集。如图4所示,AH组vs OH组在BP、MF及CC三大类中,差异表达基因所富集的GO条目分别为337、244和84条。在BP中,差异表达基因主要富集在抗原加工与提呈;在CC中,差异表达基因主要富集在主要组织相容性复合体(MHC)蛋白复合体、MHC Ⅱ类蛋白复合体和质膜蛋白复合体等;在MF中,差异表达基因主要富集在鸟苷酸结合、嘌呤核苷结合和三磷酸鸟苷结合等。
图4 牦牛犊牛结肠差异表达基因GO功能富集分析(AH组vs OH组)

1:抗原处理与呈递 antigen processing and presentation;2:免疫反应 immune response;3:免疫系统过程 immune system process;4:蛋白质水解 proteolysis;5:膜组织 membrane organization;6:跨膜运输 transmembrane transport;7:脂质代谢过程 lipid metabolic process;8:硫化合物代谢过程 sulfur compound metabolic process;9:代谢过程的正向调控 positive regulation of metabolic process;10:大分子代谢过程的正向调控 positive regulation of macromolecule metabolic;11:主要组织相容性复合体蛋白复合体 MHC protein complex;12:主要组织相容性复合体II类蛋白复合体 MHC class II protein complex;13:质膜蛋白复合体 plasma membrane protein complex;14:质膜部分 plasma membrane part;15:高尔基体膜 Golgi membrane;16:高尔基体亚区室 Golgi subcompartment;17:细胞膜 plasma membrane;18:膜蛋白复合体 membrane protein complex;19:细胞外区域 extracellular region;20:线粒体内膜蛋白复合体 inner mitochondrial membrane protein complex;21:鸟苷核苷酸结合 guanyl nucleotide binding;22:嘌呤核苷结合 purine nucleoside binding;23:三磷酸鸟苷结合 GTP binding;24:核糖核苷结合 ribonucleoside binding;25:嘌呤核糖核苷结合 purine ribonucleoside binding;26:核苷结合 nucleoside binding;27:鸟苷核糖核苷酸结合 guanyl ribonucleotide binding;28:磷脂酰肌醇磷脂酶C活性 phosphatidylinositol phospholipase C activity;29:磷脂酶C活性 phospholipase C activity;30:核苷三磷酸酶活性 nucleoside-triphosphatase activity。

Fig.4 GO functional enrichment analysis of differently expressed genes in colon of yak calves (AH group vs OH group)

图5所示,AH组vs AO组在BP、MF及CC三大类中,差异表达基因所富集的GO条目分别为449、297和123条。在BP中,差异表达基因主要富集磷酸化、含核碱化合物的运输、蛋白质磷酸化等;在CC中,差异表达基因主要富集在细胞器亚区室、高尔基体亚区室和肌球蛋白复合体等;在MF中,差异表达基因主要富集在作用于酸酐的水解酶活性、含核苷化合物的跨膜转运蛋白活性和作用于酸的水解酶活性等。
图5 牦牛犊牛结肠差异表达基因GO功能富集分析(AH组vs AO组)

1:磷酸化 phosphorylation;2:含核碱化合物的运输 nucleobase-containing compound transport;3:蛋白质磷酸化 protein phosphorylation;4:依赖DNA的DNA复制 DNA-dependent DNA replication;5:DNA复制起始 DNA replication initiation;6:氮化合物运输 nitrogen compound transport;7:水解酶活性的调控 regulation of hydrolase activity;8:磷酸代谢过程的调控 regulation of phosphate metabolic process;9:三磷酸鸟苷酶活性的调控 regulation of GTPase activity;10:磷代谢过程的调控 regulation of phosphorus metabolic process;11:细胞器亚区室 organelle subcompartment;12:高尔基体亚区室 Golgi subcompartment;13:肌动蛋白复合体 myosin complex;14:高尔基体膜 Golgi membrane;15:电压门控钠通道复合体 voltage-gated sodium channel complex;16:钠通道复合体 sodium channel complex;17:核外膜-内质网膜 nuclear outer membrane-endoplasmic reticulum membrane;18:细胞骨架 cytoskeleton;19:细胞骨架部分 cytoskeletal part;20:肌动蛋白细胞骨架 actin cytoskeleton;21:作用于酸酐的水解酶活性 hydrolase activity,acting on acid anhydrides;22:含核苷化合物的跨膜转运蛋白活性 nucleoside-containing compound transmembrane transporter activity;23:作用于酸的水解酶活性 hydrolase activity, acting on acid;24:蛋白激酶活性 protein kinase activity;25:焦磷酸酶活性 pyrophosphatase activity;26:肌动蛋白结合 actin binding;27:核苷三磷酸酶活性 nucleoside-triphosphatase activity;28:三磷酸鸟苷酶活性 GTPase activity;29:蛋白质丝氨酸/苏氨酸激酶活性 protein serine/threonine kinase activity;30:钠离子跨膜转运蛋白活性 sodium ion transmembrane transporter activity。

Fig.5 GO functional enrichment analysis of differently expressed genes in colon of yak calves (AH group vs AO group)

图6所示,AO组vs OH组中在BP、MF及CC三大类中,差异表达基因所富集的GO条目分别为355、264和76条。在CC类中,差异表达基因主要富集在肌球蛋白复合体;在MF中,差异表达基因主要富集在主动跨膜转运酶活性、二级主动跨膜转运蛋白活性和共转运体活性等。
图6 牦牛犊牛结肠差异表达基因GO功能富集分析(AO组vs OH组)

1:无机阴离子运输 inorganic anion transport;2:阴离子运输 anion transport;3:免疫系统过程 immune system process;4:免疫反应 immune response;5:多细胞生物过程的调控 regulation of multicellular organismal process;6:多细胞生物发育的调控 regulation of multicellular organismal development;7:辅酶代谢过程 coenzyme metabolic process;8:吡啶核苷酸代谢过程 pyridine nucleotide metabolic process;9:烟酰胺核苷酸代谢过程 nicotinamide nucleotide metabolic process;10:含吡啶化合物的代谢过程 pyridine-containing compound metabolic process;11:肌球蛋白复合体 myosin complex;12:细胞骨架 cytoskeleton;13:肌动蛋白细胞骨架 actin cytoskeleton;14:高尔基体膜 Golgi membrane;15:细胞骨架部分 cytoskeletal part;16:高尔基体亚区室 Golgi subcompartment;17:转移酶复合体 transferase complex;18:核质 nucleoplasm;19:核质部分 nucleoplasm part;20:细胞外区域 extracellular region;21:主动跨膜转运蛋白活性 active transmembrane transporter activity;22:二级主动跨膜转运蛋白活性 secondary active transmembrane transporter activity;23:共转运蛋白活性 symporter activity;24:受体调节器活性 receptor regulator activity;25:受体配体活性 receptor ligand activity;26:跨膜转运蛋白活性 transmembrane transporter activity;27:钠离子跨膜转运蛋白活性 sodium ion transmembrane transporter activity;28:氧化还原酶活性,作用于配对供体,伴有分子氧的掺入或还原 oxidoreductase activity, acting on paired donors, with incorporation or reduction of molecular oxygen;29:细胞因子活性 cytokine activity;30:血红素结合 heme binding。

Fig.6 GO functional enrichment analysis of differently expressed genes in colon of yak calves (AO group vs OH group)

对牦牛犊牛结肠差异表达基因进行KEGG富集分析。如表3所示,AH组vs OH组的差异表达基因主要富集在细胞黏附分子、抗原加工与提呈和趋化因子信号通路等通路;AH组vs AO组的差异表达基因主要富集在趋化因子信号通路;AO组vs OH组的差异表达基因主要富集在紧密连接通路。
表3 结肠的差异表达基因及其KEGG富集通路

Table 3 Differentially expressed genes and in colon and its KEGG-enriched pathways

KEGG通路
KEGG pathways
上调差异表达
基因数目
Number of
up-regulated
DEGs
下调差异表达
基因数目
Number of
down-regulated
DEGs
主要上调
差异表达基因
Main up-
regulated
DEGs
主要下调差异
表达基因
Main down-
regulated
DEGs
AH组vs OH组AH group vs OH group
细胞黏附分子
Cell adhesion molecules
7 28 CNTN2/SLITRK6/
CDH5
CLDN2/CD6/
SPN
抗原加工与提呈
Antigen processing and presentation
6 20 NFYB RFX5/TAP2/
CD8B
趋化因子信号通路
Chemokine signaling pathway
9 17 PLCB4/GNAI1/
ROCK2
CXCR6/CCL5/
CXCL16
AO组vs AH组AO group vs AH group
趋化因子信号通路
Chemokine signaling pathway
13 41 ROCK2/ROCK1/
GNG11
CXCR6/CXCL16/
RAC2
AO组vs OH组AO group vs OH group
紧密连接
Tight junction
4 17 Claudin/Arp2/
PP2A/Occludin
LGL1

CNTN2:接触素2 contactin 2;SLITRK6:SLIT和NTRK样家族成员6 SLIT and NTRK-like family member 6;CDH5:钙黏蛋白5 cadherin 5;CLDN2:封闭蛋白2 Claudin 2;CD6:CD6分子 CD6 molecule;SPN:涎福林蛋白 sialophorin ;NFYB:核转录因子Y亚基B nuclear factor Y subunit B;RFX5:调节因子X5 regulatory factor X5;TAP2:抗原加工相关转运蛋白2 antigen processing-related transporter 2;CD8B:CD8β分子 CD8 molecule beta chain;PLCB4:磷脂酶C beta 4 phospholipase C beta 4;GNAI1:G蛋白亚基α-i1 G protein subunit alpha i1;ROCK2:Rho相关卷曲螺旋蛋白激酶2 Rho-associated coiled-coil containing protein kinase 2;CXCR6:CXC趋化因子受体6 C-X-C motif chemokine receptor 6;CCL5:C-C趋化因子配体5 C-C motif chemokine ligand 5;CXCL16:CXC趋化因子配体16 C-X-C motif chemokine ligand 16;ROCK1:Rho相关卷曲螺旋激酶1 Rho associated coiled-coil containing protein kinase 1;GNG11:G蛋白亚基γ11 G protein subunit gamma 11;RAC2:Ras相关C3肉毒杆菌毒素底物2 Ras-related C3 botulinum toxin substrate 2;Claudin:封闭蛋白 claudin;Arp2:肌动蛋白相关蛋白2 actin-related protein 2;PP2A:蛋白磷酸酶2A protein phosphatase 2A;Occludin:闭合蛋白 occludin;LGL1:大肿瘤抑制激酶1 large tumor suppressor kinase 1。

3 讨论

断奶前后是犊牛免疫调节的关键时期,肠道在这一过程中发挥了重要作用。虽然肠道不是独立的免疫器官,但它是机体免疫系统的重要组成部分,作为表面积最大、含有最多免疫细胞的结构,肠道是防止感染的第1道防线。本团队前期研究发现,混合饲喂苜蓿干草和燕麦干草能够提高空肠中干扰素-γ(IFN-γ)含量,而单一饲喂苜蓿干草则降低结肠中IFN-γ含量[5]。这些变化与肠腔内营养物质有关,受到谷氨酰胺、短链脂肪酸、益生菌等多种底物的调控[6-7]。相比单一饲喂,混合饲喂可以避免氮浪费,补充必要营养素,并有效提高肠道黏膜免疫功能[8]。干扰素-γ含量的降低会导致免疫功能障碍,而肠道固有层的分泌型免疫球蛋白A(sIgA)则通过阻断细菌和毒素的黏附,维持肠道稳态并增强黏膜屏障[9]。因此,混合饲喂苜蓿干草和燕麦干草比单一饲喂更有利于提高犊牛的整体健康和免疫功能。
基于上述的研究结果,混合饲喂苜蓿干草和燕麦干草相比于单独饲喂苜蓿干或燕麦干草提高了牦牛犊牛的终末体重和饲料转化率,同时改善了黏膜免疫功能。为探究其深层机理,本试验选择小肠和大肠的代表性肠段空肠和结肠进行转录组测序。转录组测序结果显示,各组空肠的差异表达基因主要参与了能量代谢和免疫调控等相关通路。混合干草相比于苜蓿干草,参与蛋白质消化吸收的主要基因溶质载体家族9成员A3(SLC9A3)基因的表达量升高,有助于促进钠离子的吸收,进而增强肠道对水分和营养物质的吸收能力[10],从而对动物生长性能起着积极的作用。细胞外基质(EMC)-受体互作通路和焦点黏附通路属于信号分子和相互作用过程,EMC参与细胞间信息传递等[11]。焦点黏附通路在细胞黏附等正常生理过程中起重要作用。相较于燕麦干草,饲喂苜蓿干草组参与此通路的关键基因表达量升高,说明细胞间信号活动增多,调节细胞外基质功能进而调节肠道功能[12]。抗原处理和呈递通路中,主要组织相容性复合体Ⅰ类分子(MHCⅠ)可与内源性抗原结合,启动特异性免疫[13]。本研究发现,饲喂混合干草的牦牛犊牛空肠主要组织相容性复合体Ⅱ类转录激活因子(CⅡTA)和CD8β分子(CD8B)基因的表达量升高,进而激活了MHCⅠ类免疫途径,对空肠免疫功能的增强具有重要意义。补体和凝血级联系统是先天免疫的组成部分,通过多种机制触发酶联反应[14],参与溶解靶细胞、促进吞噬作用、中和病原体等[15]。甘露糖结合凝集素相关丝氨酸蛋白酶(mannose-binding lectin-associated serine protease,MASP)是重要的天然免疫防御分子,通过激活补体和调理吞噬清除病原体[16-17]。本研究中,MASP1基因的表达量升高,预示着混合干草在牦牛犊牛抵御病原体入侵的免疫应答中起重要作用。
结肠中差异表达基因主要参与细胞黏附分子、趋化因子信号通路和紧密连接等通路。本研究发现,相比于饲喂燕麦干草,饲喂苜蓿干草能够提高细胞黏附分子通路相关基因的表达。细胞黏附分子是一类调节细胞与细胞外基质相互结合的膜表面糖蛋白,主要通过受体-配体结合,促进细胞间相互作用,是细胞应答、炎性反应、凝血、肿瘤转移及创伤愈合等过程的关键分子基础[18]。趋化因子信号传导通路在免疫、炎症和癌症转移中发挥关键作用。趋化因子C-C基序趋化因子配体5(CCL5)可以调节T细胞表达和分泌[19],CCL5在多种肠道疾病中发挥作用,如在肠易激综合征中CCL5表达增加并募集嗜酸性粒细胞;在慢性炎症过程中,CCL5表达上调,加剧炎症反应[20]。相比于燕麦干草,饲喂苜蓿干草组结肠的CCL5基因表达量降低,意味着肠道中的免疫应答相对减弱,饲喂苜蓿干草时肠道的免疫反应更为温和。相比于苜蓿干草,饲喂混合干草影响趋化因子通路的基因Rho相关卷曲螺旋蛋白激酶(ROCK)2、ROCK1表达显著上调。ROCK是Rho激酶基因,主要调控ROCK信号通路,控制细胞迁移、增殖、分化、凋亡、存活和基因转录[21]ROCK基因表达量上升,说明饲喂混合干草增强了结肠动力,促进了肠道蠕动。紧密连接是肠道屏障的关键结构,由蛋白质复合物组成,封闭细胞间隙,维持上皮细胞排列,保障肠道屏障完整性和功能。封闭蛋白(Claudin)和闭合蛋白(Occludin)基因编码的蛋白质在紧密连接的组装和维护中发挥关键作用[22]Occludin基因编码的蛋白质是肠道紧密连接的核心组分,负责维持细胞间的信号传递和囊泡转运[23]。本研究发现,混合干草通过促进肠道ClaudinOccludin基因的表达,增强肠道屏障功能,进而预防肠道疾病的发生,促进牦牛犊牛的整体健康。
综上所述,肠道转录组学的研究可以为解析肠道免疫因子间的复杂关系提供重要视角。在空肠中,混合干草组的CⅡTAMASP1等基因,可能通过多种机制影响肠道sIgA的分泌与功能。CⅡTA基因表达量升高,既增强抗原呈递促进B细胞活化分化,进而增加sIgA分泌,又通过调节Th细胞亚群分化,间接影响sIgA产生[24]MASP1基因激活补体系统,增强免疫反应,调节炎症和免疫细胞活化,进而影响sIgA分泌,其剪接变体抑制补体过度激活,间接调节免疫反应[25]。在结肠中,混合干草组的ClaudinOccludin等基因与IFN-γ关系密切,炎症或免疫应答时,其释放量增加。IFN-γ可经多种信号通路调控ClaudinOccludin基因表达,如激活Janus激酶-信号转导子和转录激活子通路,使转录因子磷酸化、激活并结合到基因启动子区域,调节转录水平[26]。肠道转录组学为理解肠道免疫调控机制提供了重要窗口,分析特定基因的表达变化及其相互作用,有助于揭示饲料影响肠道免疫的机制,并为制定科学饲养策略提供理论基础。

4 结论

与单独饲喂苜蓿干草或燕麦干草相比,二者混合饲喂能改善牦牛犊牛免疫功能,提高空肠中MASP1基因及结肠中ClaudinOccludin基因的表达量,调节肠道免疫响应能力和健康水平,有利于哺乳期牦牛犊牛的健康高质量培育。
[1]
张乃锋, 屠焰, 刁其玉. 幼龄反刍动物健康培育体系构建及其科学问题[J]. 科学通报, 2017, 62(26):2999-3007.

ZHANG N F, TU Y, DIAO Q Y. Establishment of young ruminants rearing system and its key scientific issues[J]. Chinese Science Bulletin, 2017, 62(26):2999-3007. (in Chinese)

[2]
何江峰, 王力伟, 苏少锋, 等. 饲草燕麦的营养特性及其在反刍动物生产中的应用研究进展[J]. 中国畜牧杂志, 2023, 59(6):82-86.

HE J F, WANG L W, SU S F, et al. Nutritional characteristics of oat (Avena sativa L.) and its application in ruminant production:a review[J]. Chinese Journal of Animal Science, 2023, 59(6):82-86. (in Chinese)

[3]
梅秀丽, 李钰莹, 邝良德, 等. 燕麦干草和苜蓿干草的组合效应对肉兔生长性能的影响[J]. 动物营养学报, 2023, 35(11):7335-7343.

DOI

MEI X L, LI Y Y, KUANG L D, et al. Effects of combined effects of oat hay and alfalfa hay on growth performance of meat rabbits[J]. Chinese Journal of Animal Nutrition, 2023, 35(11):7335-7343. (in Chinese)

DOI

[4]
周亚楠, 冯宇哲, 杨得玉, 等. 苜蓿干草、燕麦干草及二者混合饲喂对哺乳期牦牛犊牛生长性能、血清生化指标及瘤胃发酵参数、组织形态和微生物区系的影响[J]. 动物营养学报, 2023, 35(2):995-1007.

DOI

ZHOU Y N, FENG Y Z, YANG D Y, et al. Effects of alfalfa hay,oat hay and their mixed feeding on growth performance,serum biochemical indexes and rumen fermentation parameters,morphology and microflora of suckling yak calves[J]. Chinese Journal of Animal Nutrition, 2023, 35(2):995-1007. (in Chinese)

[5]
安乐乐, 薛国良, 周亚楠, 等. 不同粗饲料来源饲粮对哺乳期牦牛犊牛养分表观消化率、肠道组织形态、免疫指标及消化酶活性的影响[J]. 动物营养学报, 2024, 36(9):5817-5827.

DOI

AN L L, XUE G L, ZHOU Y N, et al. Effects of different roughage source diets on nutrient apparent digestibility,intestinal histomorphology,immune indices and digestive enzyme activities of pre-weaned yak calves[J]. Chinese Journal of Animal Nutrition, 2024, 36(9):5817-5827. (in Chinese)

[6]
WISCHMEYER P E, LYNCH J, LIEDEL J, et al. Glutarnine administration reduces gram-negative bacteremia in severely burned patients:a prospective,randomized,double-blind trial versus isonitrogenous control[J]. Critical Care Medicine, 2075, 29(11):2075-2080.

[7]
YANG W G, XU T M, HUANG X S, et al. Short chain fatty acids regulate T cell metabolism to promote IL-22 production and gut immunity[J]. The Journal of Immunology, 2020, 204(S1):83.4.

[8]
杨雪馨. 补饲粗饲料对哺乳期犊牛生长性能、瘤胃发酵与胃肠道微生物的影响[D]. 硕士学位论文. 杨凌: 西北农林科技大, 2022.

YANG X X. Effects of supplementary forage on growth performance,rumen fermentation and gastrointestinal tract microorganisms of pre-weaning calves[D]. Master’s Thesis. Yangling: Northwest A&F University, 2022. (in Chinese)

[9]
JIANG Y, ZHANG W H, GAO F, et al. Effect of sodium butyrate on intestinal inflammatory response to lipopolysaccharide in broiler chickens[J]. Canadian Journal of Animal Science, 2015, 95(3):389-395.

[10]
WANG J L, ZHAO L, ZHU J, et al. Expression,localization,and effect of high salt intake on electroneutral Na+/HCO-2 cotransporter NBCn2 in rat small intestine:implication in intestinal NaCl absorption[J]. Frontiers in Physiology, 2019, 10:1334.

[11]
杨璐, 张宁, 魏爽爽, 等. 细胞外基质蛋白调控多发性硬化症髓鞘再生的研究进展[J]. 宁夏医科大学学报, 2023, 45(10):1060-1064.

YANG L, ZHANG N, WEI S S, et al. Research progress of extracellular matrix protein regulating myelin regeneration in multiple sclerosis[J]. Journal of Ningxia Medical University, 2023, 45(10):1060-1064. (in Chinese)

[12]
DERAMAUD T B, DUJARDIN D, NOULET F, et al. Altering FAK-paxillin interactions reduces adhesion, migration and invasion processes[J]. PLoS One, 2014, 9(3):e92059.

[13]
FUJIO K, MISAKI Y, SETOGUCHI K, et al. Functional reconstitution of class Ⅱ MHC-restricted T cell immunity mediated by retroviral transfer of the alpha beta TCR complex[J]. Journal of Immunology, 2000, 165(1):528-532.

[14]
武娜, 王爱桃, 董海云, 等. 补体成分与凝血功能的相互作用[J]. 世界最新医学信息文摘, 2018, 18(88):82-83,85.

WU N, WANG A T, DONG H Y, et al. Effect of complement composition and coagulation function[J]. World Latest Medicine Information, 2018, 18(88):82-83,85. (in Chinese)

[15]
韩香雨, 靳玮江, 蒋元琳, 等. 补体与凝血级联激活等通路调控麝鼠香腺周期性退化过程[J]. 基因组学与应用生物学, 2022, 41(2):257-270.

HAN X Y, JIN W J, JIANG Y L, et al. Complement and coagulation cascades and other pathways regulate the process of periodic degeneration of muskrat scented glands[J]. Genomics and Applied Biology, 2022, 41(2):257-270. (in Chinese)

[16]
ZHANG S C, WANG C F, WANG Y J, et al. Presence and characterization of complement-like activity in the amphioxus Branchiostoma belcheri tsingtauense[J]. Zoological Science, 2003, 20(10):1207-1214.

[17]
王倩. 半滑舌鳎补体凝集素途径基因MASP1、MASP2和CL-11的鉴定、表达和功能分析[D]. 硕士学位论文. 青岛: 青岛大学, 2019.

WANG Q. Identification, expression and function analysis of MASP1,MASP2 and CL-11 gene of complement lectin pathway from half-smooth tongue sole (Cynoglossus semilaevis)[D]. Master’s Thesis. Qingdao: Qingdao University, 2019. (in Chinese)

[18]
刘凤茹, 侯振江, 王秀文. 细胞黏附分子[J]. 检验医学与临床, 2007, 4(8):748-750.

LIU F R, HOU Z J, WANG X W. Cell adhesion molecule[J]. Laboratory Medicine and Clinic, 2007, 4(8):748-750. (in Chinese)

[19]
张颖, 黄卫锋. 趋化因子CCL5及其受体与自身免疫性疾病的研究进展[J]. 临床和实验医学杂志, 2016, 15(21):2175-2177.

ZHANG Y, HUANG W F. Research progress on chemokine CCL5 and its receptors in autoimmune diseases[J]. Journal of Clinical and Experimental Medicine, 2016, 15(21):2175-2177. (in Chinese)

[20]
LOU X H, ZHU H T, NING L G, et al. EZH2 regulates intestinal inflammation and ptosis through the JNK signaling pathway in intestinal epithelial cells[J]. Digestive Diseases and Sciences, 2019, 64(12):3518-3527.

[21]
易春凤, 雷晴. 蛋白激酶受体2在瘙痒性皮肤病中的机制研究进展[J]. 临床科学杂志, 2023, 52(12):767-768.

YI C F, LEI Q. Research progress on the mechanism of protease-activated receptor 2 in itchy skin diseases[J]. Journal of Clinical Dermatology, 2023, 52(12):767-768. (in Chinese)

[22]
ROEHLEN N, ROCA SUAREZ A A, EL SAGHIRE H, et al. Tight junction proteins and the biology of hepatobiliary disease[J]. International Journal of Molecular Sciences, 2020, 21(3):825.

[23]
段继娇, 谢宇潇, 朱俊红, 等. Occludin基因在猪肠道屏障中的研究进展[J]. 饲料研究, 2023, 46(18):140-144.

DUAN J J, XIE Y X, ZHU J H, et al. Research progress of Occludin gene in pig intestinal barrier[J]. Feed Research, 2023, 46(18):140-144. (in Chinese)

[24]
万云霞, 吴涛, 白海. CⅡTA基因在黏膜相关淋巴组织淋巴瘤中的研究进展[J]. 国际输血及血液学杂志, 2019, 42(6):530-534.

WANG Y X, WU T, BAI H. Progress of CⅡTA gene in mucosa-associated lymphoid tissue lymphoma[J]. International Journal of Blood Transfusion and Hematology, 2019, 42(6):530-534. (in Chinese)

[25]
郭辉, 魏斐斐, 蒋群湘, 等. 广西扶绥县壮族人群MASP1基因单核苷酸多态性与肝癌遗传易感性的关系[J]. 广西医学, 2019, 41(9):1065-1068,1072.

GUO H, WEI F F, JIANG Q X, et al. Relationship between single nucleotide polymorphism of MASP1 gene and genetic susceptibility to hepatocellular carcinoma among Zhuang population in Fusui County,Guangxi[J]. Guangxi Medical Journal, 41(9):1065-1068,1072. (in Chinese)

[26]
JACQUES C, CHATELAIS M, FEKIR K, et al. The unitary micro-immunotherapy medicine interferon-γ (4 CH) displays similar immunostimulatory and immunomodulatory effects than those of biologically active human interferon-γ on various cell types[J]. International Journal of Molecular Sciences, 2022, 23(4):2314.

Outlines

/