REVIEW

Effects of Vitamin B12 on Immunological Properties of Animals and Its Application in Animal Production

  • GE Minghui ,
  • MA Yanfen ,
  • MA Yun ,
  • ZHANG Hongrui , *
Expand
  • School of Animal Science and Technology, Ningxia University, Yinchuan 750021, China
* lecturer, E-mail:

Received date: 2025-01-16

  Online published: 2025-09-12

Abstract

Vitamin B12 (VB12) is the only B vitamin that contains a metalion, and it plays a crucial role in regulating animal health. It significantly impacts various aspects of animal physiology, including immune regulation, antioxidant capacity, growth and development, and intestinal health. This review focuses on the immune regulatory mechanisms of VB12 in animals and its applications in ruminant production, aiming to provide insights into how VB12 modulates animal health and to offer references for optimizing its use in animal production strategies.

Cite this article

GE Minghui , MA Yanfen , MA Yun , ZHANG Hongrui . Effects of Vitamin B12 on Immunological Properties of Animals and Its Application in Animal Production[J]. Chinese Journal of Animal Nutrition, 2025 , 37(9) : 5794 -5801 . DOI: 10.12418/CJAN2025.471

在畜牧业现代化进程持续加速的当下,动物营养研究的重要性愈发凸显,精准把握动物营养需求已成为提升养殖效益、保障动物健康及推动畜牧业可持续发展的核心要素。维生素B12(VB12)是B族维生素中唯一含有金属离子的成员[1],主要通过参与甲硫氨酸(methionine,Met)循环和一碳代谢(one-carbon metabolism,OCM),维持DNA复制完整性,并为免疫细胞的活化与增殖提供能量支持[2-4]。研究发现,在动物生产实践中,合理补充VB12可显著提高奶牛、肉羊、母猪、肉鸡等经济动物的生长性能和免疫性能,同时改善其抗氧化能力与整体健康水平[5-8]。尽管VB12的作用机制逐渐清晰,但其在不同动物品种、不同生长阶段及生理状态下的需求量与最佳添加方式仍需进一步研究。本文综合近年来关于VB12的研究成果,详细探讨其在动物体内的免疫调节机制及其在动物生产中的应用前景,旨在为深入理解VB12在动物健康中的关键作用提供理论依据。

1 VB12概述

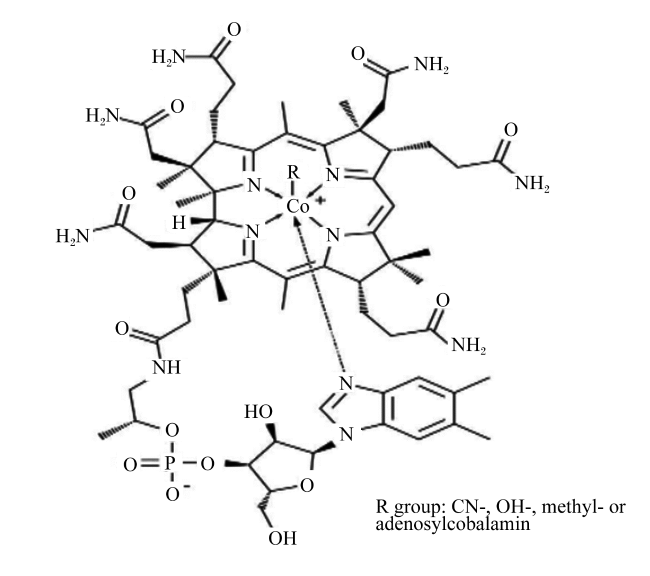
VB12又称钴胺素(cobalamin),主要由核心的咕啉环(corrin ring)、钴离子(Co3+)以及与钴离子配位的配体(如核苷酸部分)组成[1],化学结构见图1。在自然界中,VB12主要存在于动物源性食品中,肉类、肝脏、鱼类等都是其重要来源,而植物源性食物中基本不含有活性VB12[9]。研究发现,VB12作为甲硫氨酸合成酶(methionine synthase,MS)和甲基丙二酰辅酶A变位酶(methylmalonyl coenzyme-A mutase,MCM)的辅酶,在维持红细胞生成、神经髓鞘形成以及抗氧化防御系统等生理过程中具有关键作用[10-12]。分子机制研究表明,VB12可通过抑制核因子-κB(nuclear factor-kappa B,NF-κB)核转位、降低Toll样受体-4(Toll-like receptor-4,TLR-4)的表达水平和调节p38丝裂原活化蛋白激酶(p38 mitogen-activated protein kinase,p38 MAPK)磷酸化水平等途径调控先天免疫应答,提高动物免疫性能[13-15]。对于反刍动物,其瘤胃微生物可利用饲粮中的钴合成VB12,而单胃动物则依赖外源性补充[16]。特别是在动物快速生长阶段,幼龄动物因组织器官发育和代谢需求激增,对VB12的需求量显著升高[16]。如果未能及时补充VB12,则可能对幼畜的健康生长产生不利影响[16-17]。此外,妊娠期和泌乳期的母畜也需要更多的VB12,以确保其自身的健康和幼畜的正常发育[18]
图1 VB12的化学结构

R group: CN-,OH-,methyl- or adenosylcobalamin.R基团:氰基、羟基、甲基或腺苷钴胺素。

Fig.1 Chemical structure of VB12[19]

2 VB12在动物体内的消化代谢过程

VB12在动物体内的消化吸收和代谢过程是一个复杂且高度有序的过程,涉及多个器官、蛋白质和酶的协同作用[20]。VB12的吸收起始于胃部,胃酸和胃蛋白酶将VB12从食物蛋白质中释放出来,释放后的VB12与唾液腺分泌的R蛋白结合[20]。R蛋白是一种糖蛋白,能够保护VB12免受胃酸的破坏,并将其运送到小肠[20]。小肠中的胰蛋白酶和胰凝乳蛋白酶协同降解R蛋白,释放VB12。随后,VB12与胃壁细胞分泌的内因子(intrinsic factor,IF)结合[20]。IF具有特异性识别能力,能够结合具有β-配位结构(如DMB基团)的VB12活性形式,防止其被消化酶降解,并将其运送到回肠末端[20]。在回肠末端,IF-VB12复合物通过Cubam复合体(由AMN蛋白和Cubilin蛋白组成的复合物)介导的内吞作用进入肠上皮细胞[20]。Cubam复合体位于回肠末端肠上皮细胞的刷状缘,能够特异性识别并结合IF-VB12复合物,将其内吞进入细胞内部[20]
IF-VB12复合物进入细胞后,IF在溶酶体中被降解,而VB12则通过含LMBR1结构域1蛋白(LMBR1 domain containing 1,LMBRD1)的帮助穿过溶酶体膜,进入细胞质[10]。转钴胺素Ⅱ(transcobalamin Ⅱ,TCⅡ)是VB12在动物体内运输和代谢过程中的关键蛋白质。在细胞质中,VB12与TCⅡ结合,形成全转钴胺素Ⅱ(holotranscobalamin Ⅱ,HTCⅡ),此为VB12在血液中的主要运输形式,能够将VB12高效运输到全身各个组织细胞中[10]。TCⅡ对VB12具有高选择性,确保只有活性形式的VB12进入血液循环[20]。多余的VB12通过尿液排出体外,而通过胆汁排出的游离VB12需在小肠中重新与IF结合,再次通过Cubam复合体吸收,形成肠肝循环[20]。这一循环机制显著提高了VB12的利用效率,同时减少因排泄造成的损失[21]

3 VB12对动物免疫性能的调节作用机制

3.1 VB12通过NF-κB通路增强免疫应答的分子机制

研究表明,VB12通过调控OCM和Met循环影响NF-κB信号通路活性,在免疫调节中发挥重要作用。其核心作用机制涉及同型半胱氨酸(homocysteine,Hcy)代谢调控及表观遗传修饰。VB12作为MS的辅酶,催化Hcy转化为Met并生成S-腺苷甲硫氨酸(S-adenosylmethionine,SAM),后者作为通用甲基供体参与DNA甲基化调控[22]。VB12缺乏时,OCM失衡引发的Hcy蓄积及SAM/S-腺苷同型半胱氨酸(S-adenosylhomocysteine,SAH)比率下降,可通过表观遗传和氧化应激双重机制协同激活NF-κB信号通路,进而形成慢性炎症微环境[11]。Peterson等[22]研究发现,Hcy的异常堆积通过诱导DNA低甲基化修饰,解除NF-κB靶基因的抑制性甲基化调控,显著提升白细胞介素-6(interleukin-6,IL-6)、白细胞介素-8(interleukin-8,IL-8)、肿瘤坏死因子-α(tumor necrosis factor-alpha,TNF-α)等基因的转录活性。Fanny等[12]研究发现,通过激活烟酰胺腺嘌呤二核苷酸磷酸氧化酶(nicotinamide adenine dinucleotide phosphate oxidase,NOX)促进活性氧(reactive oxygen species,ROS)生成,经ROS/核因子-κB抑制蛋白激酶(IκB kinase,IKK)信号级联反应持续活化NF-κB。这种协同作用导致慢性炎症状态,与癌症发生、病毒感染及神经退行性疾病等病理过程密切相关[11-12,22]。值得注意的是,补充VB12可有效恢复SAM生成,通过重塑DNA甲基化模式抑制NF-κB转录活性,同时降低ROS水平实现双重抗炎效应[12]。在抗病毒治疗中,这种机制可增强索非布韦疗效并减轻药物性肝脏损伤[12]。在血管炎症模型中,VB12干预显著降低C反应蛋白(C reactive protein,CRP)等炎症标志物含量,证实其神经保护作用[11]。这些跨疾病研究共同揭示了VB12通过甲基代谢重编程调控NF-κB通路的分子基础,显示出其在抗炎、神经保护和代谢调控中的重要作用。
对于VB12如何通过调控NF-κB通路增强机体免疫应答在反刍动物上也进行了相关研究。Zwierzchowski等[23]研究发现,奶牛的亚临床乳房炎与VB12缺乏和炎症标志物含量的升高有关。这种炎症反应可能通过扰乱OCM和激活NF-κB来加剧疾病的发生。这与Joseph等[24]研究的结果相似,给予补充VB12的动物体内NF-κB的表达水平降低,表明VB12可能通过抑制NF-kB的活性来减轻炎症反应,从而对机体起到保护作用。在胚胎发育领域,Rodríguez-Cano等[25]通过研究揭示了VB12缺乏对胎儿的特异性影响。绵羊模型显示母体VB12不足会导致胎儿神经与心血管系统发育缺陷,这与DNA甲基化异常及NF-κB信号通路失调密切相关,进一步揭示了VB12在胎儿发育中的关键作用。

3.2 VB12通过TLR信号通路调控免疫应答的分子机制

关于VB12调控Toll样受体(Toll-like receptor,TLR)在免疫系统中的作用,已有研究揭示其在免疫调节中的重要性。Liu等[26]发现,在系统性红斑狼疮中,TCⅡ通过促进VB12摄取和Met循环,增强单核细胞增殖和TLR-4介导的炎症反应。TCⅡ的敲除则会抑制VB12的摄取和OCM,导致细胞周期停滞在G2/M期,表现为p21水平增加和细胞周期蛋白依赖性激酶1/2(cyclin-dependent kinase 1/2,CDK1/2)表达减少,同时减少脂多糖(lipopolysaccharide,LPS)诱导的炎症因子,如C-C基序趋化因子配体2(C-C motif chemokine ligand 2,CCL2)、C-X-C基序趋化因子配体10(C-X-C motif chemokine ligand 10,CXCL10)、IL-6和TNF-α的释放。此外,VB12缺乏导致的高同型半胱氨酸血症(hyperhomocysteinaemia,HHcy)中,Hcy积累通过影响DNA甲基化和组蛋白修饰改变基因表达,并可能通过与TLR-4结合激活NF-κB信号通路,加剧炎症反应和氧化应激[27]。Hayden等[28]指出,VB12是OCM的重要辅因子,参与Hcy代谢。VB12缺乏或MS功能受损会导致Hcy水平升高,引发HHcy。Hcy积累通过氧化应激和炎症反应加剧代谢综合征的病理过程,并通过间接影响TLR信号通路,特别是TLR-4表达活性,导致NF-κB的激活,进而引发炎症反应,加剧炎症反应。
Elmadfa等[29]进一步研究表明,VB12缺乏影响树突状细胞(dendritic cell,DC)的成熟和功能,DC通过TLR识别病原体。VB12缺乏导致DC分泌白细胞介素-12(interleukin-12,IL-12)、TNF-α等细胞因子减少,影响CD4+ T细胞的分化。VB12在DNA甲基化中的作用也表明,其缺乏可能导致TLR-4表达和功能异常,增加炎症或感染风险[30]。这些研究表明,VB12通过调节OCM、Met循环和表观遗传机制,间接影响TLR信号通路的活性,从而对免疫反应产生深远影响。

3.3 VB12通过调控丝裂原活化蛋白激酶(mitogen-activated protein kinase,MAPK)通路增强免疫应答的分子机制

现有研究尚未明确VB12、OCM和MAPK通路之间的直接联系,但通过分析它们在细胞周期调控、DNA合成、炎症反应及DNA甲基化等过程中的协同作用,推测三者可能产生间接关联。在乳腺癌研究中,Gálvez-Navas等[31]团队发现OCM关键基因,如蛋氨酸tRNA(methionine tRNA,MTR)、蛋氨酸合成酶还原酶(methionine synthase reductase,MTRR)的异常表达与MAPK信号通路的致癌性激活存在显著相关性,提示VB12可能通过调控OCM代谢间接调节MAPK通路活性。Kiblawi等[32]在肿瘤模型中研究发现,VB12介导的Hcy代谢失衡会引发炎症级联反应,而慢性炎症微环境通过激活MAPK信号通路促进肿瘤发生。这种机制在神经系统中呈现特殊表型,Virdi等[33]团队证实VB12通过OCM调控的表观遗传修饰可重塑MAPK通路相关基因的表达谱,其神经保护作用可能源于对p38-MAPK介导的神经元凋亡通路的双重调控——既降低促炎因子TNF-α水平,又通过Hcy代谢维持甲基化稳态。
深入解析Hcy的枢纽作用可以发现,作为VB12代谢的核心中间产物,Hcy的积累不仅通过激活NF-κB/MAPK通路加剧神经炎症,还在骨代谢障碍中通过氧化应激激活破骨细胞[34]。这种多组织效应提示VB12的调控具有系统性特征,其通过维持Hcy代谢平衡,实现对NF-κB和MAPK通路的动态调控。同时,通过调节肠道菌群增强黏膜屏障功能,减少病原体相关分子模式(pathogen-associated molecular patterns,PAMPs)的入侵,防止LPS诱导的TLR-4/NF-κB通路过度激活,这种多维调控网络最终汇聚于免疫稳态的维持[35]
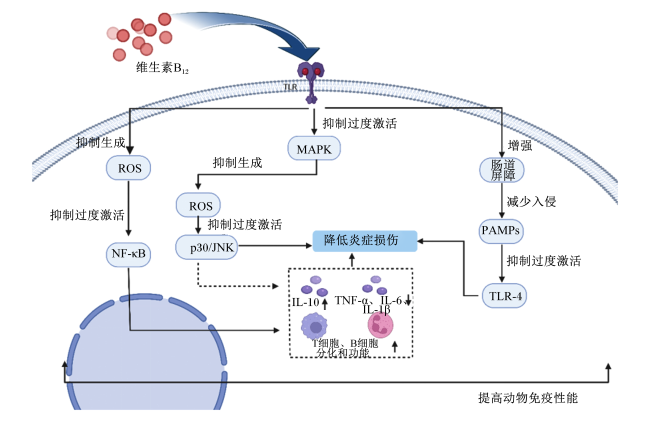
综上所述,VB12通过构建Hcy代谢-表观遗传-炎症信号的多层次调控网络,实现对NF-κB、TLR和MAPK通路的协同调节。这种作用模式不仅解释了其在抗炎、神经保护中的多靶点效应,更为理解VB12在免疫代谢重编程中的核心地位提供了理论框架。本文总结出了VB12对动物机体免疫性能的多种调节机制,见图2
图2 VB12对动物免疫性能的调控作用

ROS:活性氧reactive oxygen species;NF-κB:核因子-κB nuclear factor-κB;p38/JNK:丝裂原活化蛋白激酶p38/c-Jun氨基末端激酶 mitogen-activated protein kinase/c-Jun N-terminal kinase;MAPK:丝裂原活化蛋白激酶 mitogen-activated protein kinase;IL-10:白细胞介素-10 interleukin-10;TNF-α:肿瘤坏死因子-α tumor necrosis factor-alpha;IL-6:白细胞介素-6 interleukin-6;IL-1β:白细胞介素-1β interleukin-1 beta;T细胞:T淋巴细胞T lymphocyte;B细胞:B淋巴细胞 B lymphocyte;PAMPs:病原相关分子模式pathogen-associated molecular patterns;TLR-4:Toll样受体4 Toll-like receptor-4。

Fig.2 Regulatory functions of VB12 on animal immune function[35-36]

4 VB12在动物生产上的应用

VB12作为动物代谢的关键辅助因子,其补充效果在不同物种和生理阶段存在显著差异。研究表明,VB12通过调节甲基丙二酰辅酶A(methylmalonyl coenzyme A,MMA-CoA)代谢途径改善能量平衡、降低Hcy水平及增强抗氧化酶活性,对动物生长性能、乳/肉品质及免疫性能产生系统性优化[7,37-38]。在奶牛中,围产期补充VB12可缓解能量负平衡,降低血浆非酯化脂肪酸(non-esterified fatty acids,NEFA)和β-羟丁酸(3-hydroxybutyric acid,BHBA)含量,从而提升产奶量和乳成分[37];在肉鸡和鹅的育肥阶段,VB12则通过改善蛋白质代谢和采食量,显著提高日增重和饲料转化率[39-40]。值得注意的是,效果差异与VB12的添加方式、动物生理状态及基础饲粮钴含量密切相关[41-43]。钴供应不足时,补充VB12效果更显著,而瘤胃保护型VB12可避免微生物降解,提升利用效率[44]。具体应用参数见表1
表1 VB12在动物生产上的应用

Table 1 Application of VB12 in animal production

动物
Animals
添加时期
Adding period
添加方式
Adding ways
添加量
Supplement level
应用效果
Application effect
参考文献
References


奶牛Cows
产前60~150 d 肌肉注射 10 mg/(头·周) 奶牛体内和乳中VB12含量↑ [5]
产前21~24 d 饲粮添加 0.5 g/(d·头) 乳脂率、乳中VB12的含量↑ [45]
围产期 肌肉注射 10 mg/头(氰钴胺) 产奶量、能量代谢效率↑ [46]
围产期 肌肉注射 10 mg/(头·周) 急性相蛋白合成、免疫相关
基因表达、免疫细胞正常功能↑
[47]
犊牛Calves 出生后7~16周龄 口服结晶
肌肉注射
100 μg/(头·周)
20 μg/头
生长速度、食欲、健康水平↑
肌肉注射和口服补充均有效果↑
[48]


母羊Ewes
产前21 d~
产后21 d
肌肉注射 200 μg/只(氰钴胺) 采食量、体重、乳蛋白含量↑ [6]
妊娠前120、
40 d、产后40 d
皮下注射 12 mg/只 母羊和羔羊肝脏VB12含量、
羔羊出生重↑、羔羊死亡率↓
[18]
产前3周~分娩 饲粮添加 10 g/kg含
VB12的微藻
抗氧化能力、免疫/脂生成
相关基因表达、羔羊出生重↑
[49]
母猪Sows 配种前42 d~分娩 饲粮添加 20、100、200、
400 μg/kg DM
母猪和仔猪血浆肝脏VB12含量↑、
母猪及仔猪体内Hcy含量↓
[7]
仔猪Piglets 断奶仔猪 饲粮添加 0.06 mg/kg DM 免疫细胞功能、抗体生成↑ [50]
25~61日龄 饲粮添加 131 μg/kg DM IgG含量、免疫细胞功能维持↑ [51]


蛋鸡Layers
母鸡22~34周龄 饲粮添加 1、5、10、
20 μg/kg DM
蛋鸡孵化率、雏鸡生长速度、
10 μg/kg时产蛋率↑
[8]
30周龄~试验结束 饲粮添加 25、100 μg/kg DM 盲肠有益菌丰度↑、
腹泻率↓
[52]
鸡蛋孵化前 蛋内注射 2 μg/枚 蛋鸡孵化率、雏鸡存活率↑ [8]


肉鸡Broilers
1~40日龄 饲粮添加 0.1 mg/kg DM 平均日增重、平均日采食量、
抗氧化酶活性、血清蛋白含量↑
[53]
孵化期
第13~15天
蛋内注射 20、40 μg/枚 孵化率、饲料转化率、采食量、
血糖、总蛋白、白蛋白含量↑
[54]
肉鸭Ducks 孵化1~21 d 饲粮添加 0.033 mg/kg DM 抗体生成、免疫系统平衡↑ [55]

DM:干物质 dry matter;Hcy:同型半胱氨酸 homocysteine;IgG:免疫球蛋白 G immunoglobulin G;“↑”:提高 increase;“↓”:降低decrease。

5 小结

本文综述了VB12在动物营养与免疫中的关键作用,并总结了其在动物生产上的应用效果。VB12通过调控多个信号通路优化免疫应答,显著提高了动物的生长性能和免疫能力。然而,VB12在不同动物品种、不同生长阶段及生理状态下的需求量与最佳添加方式仍需进一步探讨。根据现有的研究结果推测,对添加量换算后得出VB12作为饲料添加剂在各类动物上的推荐添加剂量分别为:奶牛0.10~0.30 mg/kg DM、肉羊0.10~0.30 mg/kg DM、肉鸡0.02~0.04 mg/kg DM、猪0.011~0.020 mg/kg DM。未来的研究可进一步探讨VB12的最适添加量和应用方式,以实现更高效的动物生产。
[1]
RANDACCIO L, GEREMIA S, DEMITRI N, et al. Vitamin B12:unique metalorganic compounds and the most complex vitamins[J]. Molecules, 2010, 15(5):3228-3259.

[2]
MUNTEANU C, SCHWARTZ B. The relationship between nutrition and the immune system[J]. Frontiers in Nutrition, 2022,9:1082500.

[3]
LI S Y, ZHANG Q X, GAO Y Y, et al. Serum folate, vitamin B12 levels,and systemic immune-inflammation index correlate with motor performance in Parkinson’s disease:a cross-sectional study[J]. Frontiers in Neurology, 2021,12:665075.

[4]
ARIGONY A L V, DE OLIVEIRA I M, MACHADO M, et al. The influence of micronutrients in cell culture:a reflection on viability and genomic stability[J]. Biomed Research International, 2013, 2013(1):597282.

[5]
AKINS M S, BERTICS S J, SOCHA M T, et al. Effects of cobalt supplementation and vitamin B12 injections on lactation performance and metabolism of Holstein dairy cows[J]. Journal of Dairy Science, 2013, 96(3):1755-1768.

[6]
PETERS J P, ELLIOT J M. Effect of vitamin B12 status on performance of the lactating ewe and gluconeogenesis from propionate[J]. Journal of Dairy Science, 1983, 66(9):1917-1925.

[7]
SIMARD F, GUAY F, GIRARD C L, et al. Effects of concentrations of cyanocobalamin in the gestation diet on some criteria of vitamin B12 metabolism in first-parity sows[J]. Journal of Animal Science, 2007, 85(12):3294-3302.

[8]
Poultry Science Association. Poultry science[M]. Cary: Oxford University Press,1921.

[9]
OBEID R, HEIL S G, VERHOEVEN M M A, et al. Vitamin B12 intake from animal foods,biomarkers,and health aspects[J]. Frontiers in Nutrition, 2019,6:93.

[10]
SEETHARAM B, ALPERS D H. Absorption and transport of cobalamin (vitamin B12)[J]. Annual Review of Nutrition, 1982,2:343-369.

[11]
MORETTI R, PEINKHOFER C. B vitamins and fatty acids:what do they share with small vessel disease-related dementia?[J]. International Journal of Molecular Sciences, 2019, 20(22):5797.

[12]
FANNY M F, ELAWDAN K A, FAROUK S, et al. Decreasing cytotoxic effect of sofosbuvir treatment by vitamin B12 in hepatitis C virus infected cells in-vitro[J]. Global Spine Journals, 2022, 10(2):1736-1746.

[13]
VANACKER N, GIRARD C L, BLOUIN R, et al. Effects of feed restriction and supplementary folic acid and vitamin B12 on immune cell functions and blood cell populations in dairy cows[J]. Animal, 2020, 14(2):339-345.

[14]
FAMILTSEVA A, CHATURVEDI P, KALANI A, et al. Toll-like receptor 4 mutation suppresses hyperhomocysteinemia-induced hypertension[J]. American Journal of Physiology:Cell Physiology, 2016, 311(4):C596-C606.

[15]
BULAT O. Alimentatia Ca factor al mentinerii homeostaziei imune:nutrition as a factor of maintaining immune homeostasis[C]// Integrare prin cercetare si Inovare.Chisinău:Centrul Editorial-Poligrafic al Universitătii de Stat din Moldova, 2024.

[16]
GONZÁLEZ-MONTAÑA J R, ESCALERA-VALENTE F, ALONSO A J, et al. Relationship between vitamin B12 and cobalt metabolism in domestic ruminant:an update[J]. Animals, 2020, 10(10):1855.

[17]
SOBCZY Ń SKA-MALEFORA A, DELVIN E, MCCADDON A, et al. Vitamin B12 status in health and disease:a critical review.Diagnosis of deficiency and insufficiency-clinical and laboratory pitfalls[J]. Critical Reviews in Clinical Laboratory Sciences, 2021, 58(6):399-429.

[18]
GRACE N D. The effect of increasing the vitamin B12 status of Romney ewes on foetal liver vitamin B12,milk vitamin B12 and liver vitamin B12 concentrations in suckling lambs[J]. New Zealand Veterinary Journal, 1999, 47(3):97-100.

[19]
SIMONENKO S Y, BOGDANOVA D A, KULDYUSHEV N A. Emerging roles of vitamin B12 in aging and inflammation[J]. International Journal of Molecular Sciences, 2024, 25(9):5044.

[20]
RIZZO G, LAGANÀ A S. A review of vitamin B12[M]// PATELV B. Molecularnutrition. Vitamins.London: Academic Press,2020:105-129.

[21]
O’LEARY F, SAMMAN S. Vitamin B12 in health and disease[J]. Nutrients, 2010, 2(3):299-316.

[22]
PETERSON C T, RODIONOV D A, OSTERMAN A L, et al. B vitamins and their role in immune regulation and cancer[J]. Nutrients, 2020, 12(11):3380.

[23]
ZWIERZCHOWSKI G, HAXHIAJ K, WÓJCIK R, et al. Identifying predictive biomarkers of subclinical mastitis in dairy cows through urinary metabotyping[J]. Metabolites, 2024, 14(4):205.

[24]
JOSEPH MARTIN S, EVAN PRINCE S. Comparative modulation of levels of oxidative stress in the liver of anti-tuberculosis drug treated wistar rats by vitamin B12,beta-carotene,and spirulina fusiformis:role of NF-κB,iNOS,IL-6,and IL-10[J]. Journal of Cellular Biochemistry, 2017, 118(11):3825-3833.

[25]
RODRÍGUEZ-CANO A M, CALZADA-MENDOZA C C, ESTRADA-GUTIERREZ G, et al. Nutrients,mitochondrial function,and perinatal health[J]. Nutrients, 2020, 12(7):2166.

[26]
LIU B Y, LI A, LIU Y, et al. Transcobalamin 2 orchestrates monocyte proliferation and TLR4-driven inflammation in systemic lupus erythematosus via folate one-carbon metabolism[J]. Frontiers in Immunology, 2024,15:1339680.

[27]
PERŁA-KAJÁN J, JAKUBOWSKI H. Dysregulation of epigenetic mechanisms of gene expression in the pathologies of hyperhomocysteinemia[J]. International Journal of Molecular Sciences, 2019, 20(13):3140.

[28]
HAYDEN M R. Overview and new insights into the metabolic syndrome:risk factors and emerging variables in the development of type 2 diabetes and cerebrocardiovascular disease[J]. Medicina, 2023, 59(3):561.

[29]
ELMADFA I, MEYER A L. The role of the status of selected micronutrients in shaping the immune function[J]. Endocrine,Metabolic & Immune Disorders Drug Targets, 2019, 19(8):1100-1115.

[30]
TAKAHASHI K. Influence of bacteria on epigenetic gene control[J]. Cellular and Molecular Life Sciences, 2014, 71(6):1045-1054.

DOI PMID

[31]
GÁLVEZ-NAVAS J M, MOLINA-MONTES E, RODRÍGUEZ-BARRANCO M, et al. Molecular mechanisms linking genes and vitamins of the complex B related to one-carbon metabolism in breast cancer:an in silico functional database study[J]. International Journal of Molecular Sciences, 2024, 25(15):8175.

[32]
KIBLAWI R, HOLOWATYJ A N, GIGIC B, et al. One-carbon metabolites, B vitamins and associations with systemic inflammation and angiogenesis biomarkers among colorectal cancer patients:results from the colocare study[J]. British Journal of Nutrition, 2020, 123(10):1187-1200.

[33]
VIRDI S, MCKEE A M, NUTHI M, et al. The role of one-carbon metabolism in healthy brain aging[J]. Nutrients, 2023, 15(18):3891.

[34]
ODKHUU E, NARMANDAKH S, ZINAMYADAR M, et al. Vitamin regulation of osteoclast differentiation[J]. Central Asian Journal of Medical Sciences, 2020, 6(3):114-128.

[35]
ZHANG Y F, YANG H, HOU S, et al. Influence of the brain-gut axis on neuroinflammation in cerebral ischemia-reperfusion injury (review)[J]. International Journal of Molecular Medicine, 2024, 53(3):30.

[36]
HESAMIAN M S, SHAYGANNEJAD V, GOLABI M, et al. The role of cobalamin on interleukin 10,osteopontin,and related microRNAs in multiple sclerosis[J]. Iranian Journal of Allergy,Asthma,and Immunology, 2022, 21(3):332-343.

[37]
XU N N, YANG D T, ZHANG B X, et al. Short communication:influence of intramuscular injection of vitamin B12 in early-lactation dairy cows on Mozzarella cheese quality and vitamin B12 stability[J]. Journal of Dairy Science, 2020, 103(11):9835-9840.

[38]
MOUSAVI S R, FATAHNIA F, TAASOLI G, et al. Effect of injection of vitamin E and selenium solution and vitamin B12 and iron solution to transition dairy cows on colostrum quality,and antioxidant capacity and? serum metabolites in calves[J]. Iranian Journal of Animal Science, 2020, 50(4):307-317.

[39]
LIU Y J, ZHANG J, WANG C, et al. Effects of folic acid and cobalt sulphate supplementation on growth performance,nutrient digestion,rumen fermentation and blood metabolites in Holstein calves[J]. British Journal of Nutrition, 2022, 127(9):1313-1319.

[40]
YIN H C, HUANG J. Effects of soybean meal replacement with fermented alfalfa meal on the growth performance,serum antioxidant functions,digestive enzyme activities,and cecal microflora of geese[J]. Journal of Integrative Agriculture, 2016, 15(9):2077-2086.

[41]
ARDALI M A, ANDARZGOO F, NAZARI S. Application of vitamins B1 and B12 injection on milk yield and composition and some blood biochemical traits in Holstein dairy cows[J]. Revista Brasileira de Higiene e Sanidade Animal, 2025, 19(1):1-9.

[42]
RIBEIRO T L M, FRANCIS F L, HELDT J S, et al. Evaluation of a ruminally protected blend of pantothenic acid,pyridoxine,folic acid,biotin,and vitamin B12 on finishing steer growth performance,efficiency of dietary net energy utilization,carcass trait responses,and liver abscess prevalence and severity[J]. Translational Animal Science, 2023, 7(1):txad084.

[43]
CUEVAS REYES V, SANTIAGO HERNANDEZ F, FLORES NAJERA M J, et al. Intake of spineless cladodes of Opuntia ficus-indica during late pregnancy improves progeny performance in underfed sheep[J]. Animals, 2020, 10(6):995.

[44]
BRISSON V. Mathematical modelling to predict B-vitamins supply in dairy cows[D]. Master’s Thesis. Canada: University of Guelph, 2022.

[45]
GRAULET B, MATTE J J, DESROCHERS A, et al. Effects of dietary supplements of folic acid and vitamin B12 on metabolism of dairy cows in early lactation[J]. Journal of Dairy Science, 2007, 90(7):3442-3455.

[46]
DUPLESSIS M, LAPIERRE H, SAUERWEIN H, et al. Combined biotin,folic acid,and vitamin B12 supplementation given during the transition period to dairy cows:part Ⅰ.Effects on lactation performance,energy and protein metabolism,and hormones[J]. Journal of Dairy Science, 2022, 105(8):7079-7096.

[47]
OUATTARA B, BISSONNETTE N, DUPLESSIS M, et al. Supplements of vitamins B9 and B12 affect hepatic and mammary gland gene expression profiles in lactating dairy cows[J]. BMC Genomics, 2016, 17(1):640.

[48]
DRAPER H H, SIME J T, JOHNSON B C. A study of vitamin B12 deficiency in the calf[J]. Journal of Animal Science, 1952, 11(2):332-340.

[49]
EL-SAYED A, EBISSY E, ATEYA A. Positive impacts of Nannochloropsis oculata supplementation on gene expression of immune and antioxidant markers and metabolic profile of Barki sheep in the transition period and lipogenic effects on progeny[J]. Veterinary Research Communications, 2024, 48(4):2207-2226.

[50]
YAN H, JIN J Q, YANG P, et al. Fermented soybean meal increases nutrient digestibility via the improvement of intestinal function,anti-oxidative capacity and immune function of weaned pigs[J]. Animal, 2022, 16(6):100557.

[51]
VADOPALAS L, BADARAS S, RUZAUSKAS M, et al. Influence of the fermented feed and vaccination and their interaction on parameters of large white/norwegian landrace piglets[J]. Animals, 2020, 10(7):1201.

[52]
WANG R, BAI Y, YANG Y, et al. A comparison of production performance,egg quality,and cecal microbiota in laying hens receiving graded levels of vitamin B12[J]. Frontiers in Veterinary Science, 2021,8:712183.

[53]
SAVARAM V R R, RAJU MANTENA V L N, BHUKYA P, et al. Effect of methyl donors supplementation on performance,immune responses and anti-oxidant variables in broiler chicken fed diet without supplemental methionine[J]. Animal Bioscience, 2022, 35(3):475-483.

[54]
TEYMOURI B, GHIASI GHALEHKANDI J, HASSANPOUR S, et al. Effect of in ovo feeding of the vitamin B12 on hatchability,performance and blood constitutes in broiler chicken[J]. International Journal of Peptide Research and Therapeutics, 2020, 26(1):381-387.

[55]
ALAGAWANY M, ELNESR S S, FARAG M R, et al. Nutritional significance of amino acids,vitamins and minerals as nutraceuticals in poultry production and health—a comprehensive review[J]. Veterinary Quarterly, 2021, 41(1):1-29.

Outlines

/