RESEARCH PAPER

Effects of Mulberry Leaf Polysaccharide Supplementation in High Starch Diet on Growth Performance, Antioxidant Capacity, Glucose and Lipid Metabolism, and Intestinal Microbiota of Largemouth Bass (Micropterus salmoides)

  • ZHOU Donglai , 1 ,
  • FU Bing 1 ,
  • ZHONG Wenhao 1, 2 ,
  • LI Qingrong 1 ,
  • LI Erna 1 ,
  • LI Qian 1 ,
  • YANG Qiong 1 ,
  • CHEN Bing 3 ,
  • LIAO Sentai 1 ,
  • XING Dongxu , 1, **
Expand
  • 1 Guangdong Key Laboratory of Agricultural Products Processing, Sericultural & Agri-Food Research Institute, Guangdong Academy of Agricultural Sciences, Guangzhou 510610, China
  • 2 College of Food Science and Technology, Guangdong Ocean University, Zhanjiang 524088, China
  • 3 Key Laboratory of Animal Nutrition and Feed Science in South China, Ministry of Agriculture and Rural Affairs, Guangdong Key Laboratory of Animal Breeding and Nutrition, Institute of Animal Science, Guangdong Academy of Agricultural Sciences, Guangzhou 510640, China
** professor, E-mail:

* Contributed equally

Received date: 2025-05-08

  Online published: 2025-12-13

Abstract

This study was conducted to investigate the effects of mulberry leaf polysaccharide (MLP) supplementation in high starch diet on growth performance, antioxidant capacity, glucose and lipid metabolism, and intestinal microbiota of largemouth bass (Micropterus salmoides). A total of 270 largemouth bass with an initial weight of (35.34±0.52) g were randomly divided into three groups as low starch group (CK group, 7.58% starch in diet), high starch group (HD group, 12.68% starch in diet), and high starch supplemented with MLP group (MLP group, 12.68% starch supplemented with 0.6% MLP in diet), with 3 replicates per group and 30 fish per replicate, and fed for 60 d. The results showed as follows: 1) compared to the HD group, the MLP group showed a significant increase in weight gain rate and condition factor (P<0.05), and a significant decrease in viscerosomatic index, hepatosomatic index, and feed coefficient (P<0.05). 2) Compared to the HD group, the MLP group exhibited a significant decrease in serum alanine aminotransferase and aspartate aminotransferase activities, liver malondialdehyde content, and the mRNA relative expression levels of liver interleukin-8, nuclear factor-κB, and tumor necrosis factor-α (P<0.05); a significant increase in liver total superoxide dismutase and glutathione peroxidase activities, and the mRNA relative expression levels of interleukin-10 and transforming growth factor-β (P<0.05). 3) Compared to the HD group, the MLP group showed a significant decrease in serum triglyceride (TG) and glucose contents, liver TG and glycogen contents, and the mRNA relative expression levels of liver diacylglycerol acyltransferase, fatty acid synthase, and acetyl-CoA carboxylase (P<0.05); a significant increase in the mRNA relative expression levels of liver phosphofructokinase, glucokinase, carnitine palmitoyltransferase 1, and peroxisome proliferator-activated receptor α (P<0.05). 4) Compared to the HD group, the MLP group exhibited a significant increase in intestinal muscle layer thickness and propionic acid content (P<0.05), and an upward trend in the Shannon index, Simpson index, and the relative abundances of Bacteriodota, Firmicutes, and Lactobacillus in the intestinal microbiota (P>0.05). In summary, the high starch diet supplemented with MLP can enhance the growth performance, antioxidant capacity, intestinal microbiota diversity, and beneficial bacterial relative abundance of Micropterus salmoides. It also alleviates the liver inflammation and promotes the glucose and lipid metabolism by accelerating carbohydrate and fatty acid oxidation and inhibiting insulin resistance.

Cite this article

ZHOU Donglai , FU Bing , ZHONG Wenhao , LI Qingrong , LI Erna , LI Qian , YANG Qiong , CHEN Bing , LIAO Sentai , XING Dongxu . Effects of Mulberry Leaf Polysaccharide Supplementation in High Starch Diet on Growth Performance, Antioxidant Capacity, Glucose and Lipid Metabolism, and Intestinal Microbiota of Largemouth Bass (Micropterus salmoides)[J]. Chinese Journal of Animal Nutrition, 2025 , 37(12) : 8514 -8529 . DOI: 10.12418/CJAN2025.693

大口黑鲈(Micropterus salmoides)具有生长快、肉质细腻等特点,是我国主要的经济养殖鱼类之一。淀粉作为饲料主要的能量来源和制作膨化饲料不可或缺的原料,在水产饲料中扮演着重要角色[1]。然而,许多关于大口黑鲈的研究表明,长期投喂超过10%淀粉含量的饲料会降低大口黑鲈的消化率,引起糖原和脂质沉积,并诱导炎症反应、氧化应激和免疫低下,抑制其生长[2-4]。化学合成的α-葡萄糖苷酶抑制剂虽能达到降血糖的效果,但毒性大、成本高、作用单一[5],亟需寻求天然、健康和高效的饲料添加剂来保护鱼体健康。
桑叶多糖(mulberry leaf polysaccharide,MLP)是脱脂桑叶经热水提取(超声辅助)或酶辅助提取后制得的天然植物多糖,主要组成成分为半乳糖、阿拉伯糖、鼠李糖和葡萄糖(glucose,GLU),具有无毒、无残留和高效等特点[6]。研究表明,MLP通过上调胰岛细胞中抗凋亡的B细胞淋巴瘤-2(Bcl-2)、胰腺-十二指肠同源框-1(PDX-1)、葡萄糖激酶(GK)和葡萄糖转运蛋白2(GLUT2)的表达以及促进胰岛素的分泌,调节糖尿病小鼠肝脏的GLU代谢[7]。陈晓兰等[8]发现,MLP能通过激活Toll样受体4(TLR4)/髓样分化因子88(MyD88)/p65信号通路,改变小鼠肠道微生物群落结构,修复肠道屏障功能,以及调节免疫细胞因子来拮抗免疫抑制。目前鲜有研究探寻化合物形式的MLP对水产动物中的影响,而是通常以桑叶提取物的形式添加,如鲫鱼(Carassius auratus gibelio)饲料中添加60 g/kg的桑叶提取物(换算成多糖添加量为18 g/kg)能显著提高其消化吸收能力,从而促进生长[9];添加12 g/kg的桑叶提取物能改善花鲈(Lateolabrax maculatus)肝脏功能和肠道菌群组成[10-11];添加10 g/kg的桑叶醇提取物(换算成多糖添加量为5.1 g/kg)能提高鳜鱼(Siniperca chuatsi)抗氧化能力和促进肠道发育,而不影响生长性能[12]。但这可能是桑叶提取物中各种活性成分相互作用的结果,MLP对鱼类真正的效用尚不明确。因此,本研究以大口黑鲈为试验对象,研究高淀粉饲料中添加MLP对大口黑鲈生长性能、抗氧化能力、糖和脂代谢以及肠道菌群的影响,旨在为MLP在水产动物配合饲料中的应用提供依据。

1 材料与方法

1.1 试验饲料

本试验以秘鲁鱼粉、大豆浓缩蛋白和去皮豆粕为主要蛋白质源,以鱼油、大豆油和大豆磷脂油为主要脂肪源,配制3种试验饲料。其中,低淀粉组(CK组)饲料淀粉含量为7.58%;高淀粉组(HD组)饲料淀粉含量为12.68%;高淀粉添加桑叶多糖组(MLP组)饲料淀粉含量为12.68%,并在饲料中添加0.60% MLP。MLP为市购产品,纯度约为70%。所有饲料原料粉碎后过60目筛,按表1配比称重、混匀,用102 ℃水蒸气调节8 min,然后挤压成3 mm颗粒,55 ℃烘干,置于-20 ℃保存备用。试验饲料组成及营养水平见表1
表1 试验饲料组成及营养水平(干物质基础)

Table 1 Composition and nutrient levels of experimental diets (DM basis) %

项目
Items
组别Groups
CK HD MLP
原料Ingredients
秘鲁鱼粉Peruvian fish meal 40.00 40.00 40.00
大豆浓缩蛋白Soy protein concentrate 15.00 15.00 15.00
血粉Blood meal 4.00 4.00 4.00
去皮豆粕Dehulled soybean meal 17.00 17.00 17.00
小麦淀粉Wheat starch 7.00 13.00 13.00
磷酸二氢钙Ca(H2PO4)2 1.00 1.00 1.00
维生素预混料Vitamin premix1) 0.20 0.20 0.20
矿物元素预混料Mineral premix2) 0.80 0.80 0.80
胆碱Choline 0.40 0.40 0.40
大豆磷脂油Soy lecithin oil 2.00 2.00 2.00
大豆油Soybean oil 3.00 3.00 3.00
鱼油Fish oil 3.00 3.00 3.00
桑叶多糖Mulberry leaf polysaccharides 0.60
微晶纤维素Microcrystalline cellulose 6.60 0.60
合计Total 100.00 100.00 100.00
营养水平Nutrient levels3)
粗蛋白质Crude protein 47.50 47.80 47.78
粗脂肪Crude lipid 11.70 11.78 11.74
粗灰分Crude ash 13.80 13.87 13.84
淀粉Starch 7.58 12.68 12.68

1)每千克维生素预混料含有 Each kilogram of the vitamin premix contained the following:VA 66 666 666.7 IU,VD 400 000 000 IU,VE 1 g,VK 2 g,VB1 5 g,VB2 5 g,VB6 5 g,VB12 1 g,泛酸钙 calcium pantothenate 20 g,叶酸 folic acid 10 g,生物素 biotin 1 g,烟酸 niacin 20 g,氯化胆碱 choline chloride 200 g,脱脂米糠 defatted rice bran 700 g。

2)每千克矿物元素预混料含有 Each kilogram of the mineral premix contained the following:CuCO3 4 g,FeC6H5O7 15 g,MgO 26 g,MnSO4 5 g,KCl 250 g,ZnSO4 50 g,NaCl 50 g,沸石粉 zeolite powder 600 g。

3)营养水平为实测值。Nutrient levels were measured values.

1.2 试验设计和饲养管理

试验所用大口黑鲈由广东梁氏水产种业有限公司提供,在广东省农业科学院蚕业与农产品加工研究所室内循环水养殖系统中暂养1周,暂养期间每天用CK组饲料饲喂2次。暂养结束后禁食24 h,挑选平均初始体重为(35.34±0.52) g的幼鱼270尾,随机分到9个直径为75 cm的养殖桶中(养殖水体为350 L),每桶30尾,将9个养殖桶随机分成3组,每组3个重复。试验期为60 d,期间每天表观饱食投喂2次试验饲料(09:00和16:30各1次),投喂后0.5 h将未摄食完的饲料捞出,烘干水分后称量,准确记录每天饲料采食量和试验鱼死亡情况。试验期间每周换水3次,每次换水量为每个养殖桶水量的1/3,养殖期间水温为25.4~30.2 ℃,溶氧量≥6.5 mg/L,亚硝酸盐含量≤0.05 mg/L,氨氮含量≤0.2 mg/L,pH为6.5~8.0,采取自然光照。动物试验经广东省农业科学院动物福利伦理委员会批准(批准号:GDAAS2022015)。

1.3 样本采集

饲养试验结束后,禁食24 h,统计每个重复试验鱼的数量、总重量和总摄食量,计算终末体重、增重率(weight gain rate,WGR)、特定生长率(specific growth rate,SGR)和饲料系数(feed coefficient,FCR);每个重复随机取9尾试验鱼测定体长和体重,计算肥满度(condition factor,CF),随后尾静脉采血,4 ℃静置2 h,1 324×g离心10 min,取上清液测定血清生化指标;分离内脏和肝脏并称重,计算脏体比(viscerosomatic index,VSI)和肝体比(hepatosomatic index,HSI);每个重复随机取6尾试验鱼,在无菌操作台冰上解剖后,取全肠和肝脏于-80 ℃冰箱保存,用于肠道菌群、短链脂肪酸含量以及肝脏生化和抗氧化指标、糖和脂代谢以及炎症相关基因表达测定;每个重复随机另取3尾试验鱼的中肠和肝脏分别固定于4%多聚甲醛,用于组织切片分析。

1.4 指标测定

1.4.1 饲料营养水平

饲料中粗蛋白质、粗脂肪、粗灰分和淀粉含量的测定分别参照GB/T 6432—2018、GB/T 6433—2006、GB/T 6438—2007和GB/T 42491—2023中方法进行。

1.4.2 生长性能

生长性能指标计算公式如下:
WGR(%)=100×(Wf-Wi)/Wi;
SGR(%/d)=100×(lnWf-lnWi)/T;
摄食量(feed intake,FI,g/尾)=Ft/[(Mi+Mf)/2];
FCR=Ft/(Wft-Wit);
CF(g/cm3)=100×Wf/Lf3;
VSI(%)=100×Wv/Wf;
HSI(%)=100×Wh/Wf
式中:Wi为初始体重;Wf为终末体重;T为养殖时间;Ft为总摄食量;Mi为初始尾数;Mf为终末尾数;Wft为终末总重;Wit为初始总重;Lf为终末体长;Wv为内脏团湿重;Wh为肝脏湿重。

1.4.3 血清、肝脏生化和抗氧化指标测定

根据试剂盒制造商说明书操作步骤,采用南京建成生物工程研究所商业试剂盒测定血清甘油三酯(triglyceride,TG)和GLU含量以及丙氨酸氨基转移酶(alanine aminotransferase,ALT)和天门冬氨酸氨基转移酶(aspartate aminotransferase,AST)活性。
肝脏生化和抗氧化指标测定方法如下:称取0.1 g肝脏组织,加入9倍重量生理盐水,4 ℃充分研磨后,573×g离心10 min,取上清液测定总超氧化物歧化酶(total superoxide dismutase,T-SOD)和谷胱甘肽过氧化物酶(glutathione peroxidase,GSH-Px)活性以及TG和丙二醛(malondialdehyde,MDA)含量。称取0.1 g肝脏组织,加入9倍重量生理盐水,4 ℃充分研磨后,13 201×g离心5 min,取上清液测定总抗氧化能力(total antioxidant capacity,T-AOC)。取肝脏组织,用4 ℃生理盐水润洗后,滤纸吸干水分,准确称取0.08 g肝脏组织置于试管,加入3倍肝脏重量的浓碱液,沸水浴煮20 min,流水冷却;然后加入96倍肝脏重量的双蒸水,制成检测液后进行糖原(glycogen,GLY)含量测定,具体操作步骤严格按照南京建成生物工程研究所商业试剂盒说明书进行。

1.4.4 肠道和肝脏组织切片分析

取中肠和肝脏块,小心剥离脂肪,用4 ℃生理盐水润洗后分别固定于4%多聚甲醛。肠道和肝脏组织切片制作、苏木精-伊红(HE)染色和分析参照符兵等[13]的方法。

1.4.5 肠道短链脂肪酸含量

肠道短链脂肪酸含量采用气相色谱仪(GC-2010 PLUS,岛津,日本)测定。取剪碎的肠道组织0.2 g于2 mL离心管中,加入1 mL的10 mmol/L氢氧化钠溶液(含5 mmol/L巴豆酸溶液),振荡混匀30 s,13 201×g离心2 min,取上清液过0.22 μm膜,-20 ℃过夜。
色谱条件参照Hu等[14]的报道并稍作修改。色谱柱为DB-FFAP色谱柱(30 m×0.25 mm,0.25 μm),以氮气和氢气为载气,分流比为1∶10,流速设置为30.0 mL/min,进样器和检测器温度均设置为240 ℃。

1.4.6 肠道菌群分析

用试剂盒提取肠道组织DNA后,以16S rDNA“V3+V4”高变区的序列设计引物,进行肠道菌群总DNA的PCR扩增,所用引物为338F(5'-ACTCCTACGGGAGGCAGCAG-3')和806R(5'-GGACTACHVGGGTWTCTAAT-3')。采用MiSeq高通量测序得到的PE reads首先根据overlap关系进行拼接,同时对序列质量进行质控和过滤。区分样本后进行操作分类单元(OTU)聚类分析和物种分类学注释,基于OTU进行群落组成、α多样性和β多样性统计分析[15]

1.4.7 肝脏糖和脂代谢以及炎症相关基因表达

采用RNA Easy Fast动物组织总RNA提取试剂盒[天根生化科技(北京)有限公司]从肝脏组织样品中提取总RNA,检测浓度和纯度后,用FastKing RT Kit反转录试剂盒[天根生化科技(北京)有限公司]制备cDNA模板。白细胞介素-8(IL-8)、白细胞介素-10(IL-10)、核因子-κB(NF-κB)、肿瘤坏死因子-α(TNF-α)、转化生长因子-β(TGF-β)、GK、磷酸果糖激酶(PFK)、乙酰辅酶A羧化酶(ACC)、二酰基甘油酰基转移酶(DGAT)、脂肪酸合成酶(FAS)、肉碱棕榈酰转移酶1(CPT1)、过氧化物酶体增殖物激活受体α(PPARα)和β-肌动蛋白(β-actin)引物由生工生物工程(上海)股份有限公司合成,引物信息见表2。实时荧光定量PCR反应条件为95 ℃预变性3 min,95 ℃变性10 s,60 ℃退火30 s,72 ℃延伸60 s,40个循环。以β-肌动蛋白为内参基因,采用2-△△Ct[16]计算目标基因mRNA相对表达量。
表2 实时荧光定量PCR引物信息

Table 2 Real-time fluorescence quantitative PCR primer information

基因
Genes
引物序列
Primer sequences (5'—3')
GenBank登录号
GenBank accession number
白细胞介素-8
IL-8
F:ACTTCTCCTGGCTGCTCTG
R:ACTTCTCATTTGGTTTGACACA
XM_038704089.1
白细胞介素-10
IL-10
F:CGGCACAGAAATCCCAGAGC
R:CAGCAGGCTCACAAAATAAACATCT
XM_038696252.1
核因子-κB
NF-κB
F:AGAAGACGACTCGGGGATGA
R:GCTTCTGCAGGTTCTGGTCT
XM_038699793.1
肿瘤坏死因子-α
TNF-α
F:AAATAGTGATTCCTCAAGACGG
R:TGAACAGTATGGCTCAGATGG
XM_038723994.1
转化生长因子-β
TGF-β
F:GCTTCAGTTTCGGCATTT
R:TCTCCGTGGAGCGTTTT
XM_038693206.1
葡萄糖激酶
GK
F:CTCGCTCTGCTCGTATGT
R:CTCCCTTCCTCCGACTG
XM_038703172.1
磷酸果糖激酶
PFK
F:TGGGCTATGATACAAGAGTGA
R:CCATTAGAGGCAGACGAAC
XM_038720351.1
乙酰辅酶A羧化酶
ACC
F:AAGTCCAAGAGGGCACG
R:ACTGGGAGTCCGCAAAT
XM_038704615.1
二酰基甘油酰基转移酶
DGAT
F:GCAACATCAAGCCGTCCGACTC
R:AGCACAGCGAGCCAGAGGTAAT
XM_038705876.1
脂肪酸合成酶
FAS
F:TTACACTGCCACAGCAACCA
R:TGCCCCTCCTACTACACCTC
XM_038735140.1
肉碱棕榈酰转移酶1
CPT1
F:GATGTTTTATGACGGGCGG
R:TAGGTTTCACGAGCATTGGC
XM_038705335.1
过氧化物酶体增殖物激活受体α
PPARα
F:CCACCGCAATGGTCGATATG
R:TGCTGTTGATGGACTGGGAAA
XM_038705497.1
β-肌动蛋白
β-actin
F:TTCACCACCCACAGCCGAAAG
R:TCTGGGCAACGGAACCTCT
XM_038695351.1

1.5 数据统计分析

采用SPSS 22.0软件对试验数据进行单因素方差分析(one-way ANOVA),差异显著时采用SNK法进行组间多重比较,结果以“平均值±标准误(mean±SE)”形式表示,差异显著水平为P<0.05。

2 结果与分析

2.1 高淀粉饲料中添加MLP对大口黑鲈生长性能的影响

表3可知,与HD组相比,CK组和MLP组大口黑鲈终末体重、WGR和CF显著提高(P<0.05),VSI和HSI显著降低(P<0.05);与HD组相比,MLP组FCR显著降低(P<0.05)。各组之间SGR和FI无显著差异(P>0.05)。
表3 高淀粉饲料中添加MLP对大口黑鲈生长性能的影响

Table 3 Effects of MLP supplementation in high starch diet on growth performance of Micropterus salmoides

项目
Items
组别Groups
CK HD MLP
初始体重IBW/g 36.20±1.18 35.33±0.67 34.50±0.87
终末体重FBW/g 197.92±4.84b 170.08±2.12a 196.59±5.93b
增重率WGR/% 456.31±16.25b 381.99±4.37a 471.37±31.10b
特定生长率SGR/(%/d) 2.83±0.08 2.62±0.02 2.99±0.14
脏体比VSI/% 6.33±0.58a 9.26±0.42b 7.13±0.17a
肝体比HSI/% 1.82±0.11a 2.48±0.10b 1.79±0.12a
肥满度CF/(g/cm3) 2.35±0.07b 1.85±0.04a 2.28±0.02b
饲料系数FCR 1.13±0.06ab 1.19±0.02b 1.00±0.04a
摄食量FI/(g/尾) 146.93±3.44 145.97±1.83 150.81±1.47

同行数据肩标不同字母表示差异显著(P<0.05),相同字母或无字母表示差异不显著(P>0.05)。下表同。

In the same row, values with different letter superscripts indicated significant difference (P<0.05), while with the same letter or no letter superscripts indicated no significant difference (P>0.05). The same as below.

2.2 高淀粉饲料中添加MLP对大口黑鲈血清生化指标的影响

表4可知,与HD组相比,CK组和MLP组大口黑鲈血清TG和GLU含量以及ALT和AST活性显著降低(P<0.05);与CK组相比,MLP组血清GLU含量显著降低(P<0.05)。
表4 高淀粉饲料中添加MLP对大口黑鲈血清生化指标的影响

Table 4 Effects of MLP supplementation in high starch diet on serum biochemical indices of Micropterus salmoides

项目
Items
组别Groups
CK HD MLP
甘油三酯TG/(mmol/L) 3.18±0.19a 5.65±0.41b 2.75±0.13a
葡萄糖GLU/(mmol/L) 8.98±0.36b 14.18±0.42c 4.25±0.15a
丙氨酸氨基转移酶ALT/(U/L) 40.49±1.84a 50.65±2.02b 37.51±1.95a
天门冬氨酸氨基转移酶AST/(U/L) 32.81±1.73a 43.62±1.81b 35.08±2.72a

2.3 高淀粉饲料中添加MLP对大口黑鲈肝脏生化和抗氧化指标的影响

表5可知,与HD组相比,CK组和MLP组大口黑鲈肝脏TG、GLY和MDA含量显著降低(P<0.05),肝脏T-SOD、GSH-Px活性及T-AOC显著提高(P<0.05);与CK组相比,MLP组肝脏T-AOC显著提高(P<0.05)。
表5 高淀粉饲料中添加MLP对大口黑鲈肝脏生化和抗氧化指标的影响

Table 5 Effects of MLP supplementation in high starch diet on liver biochemical and antioxidant indices of Micropterus salmoides

项目
Items
组别Groups
CK HD MLP
生化指标Biochemical indices
甘油三酯TG/(mmol/g prot) 25.48±2.44a 37.42±1.33b 29.91±2.34a
糖原GLY/(mg/g) 7.68±0.23a 10.62±0.54b 7.95±0.57a
抗氧化指标Antioxidant indices
总超氧化物歧化酶T-SOD/(U/mg prot) 10.64±0.65b 7.92±0.20a 11.16±0.48b
谷胱甘肽过氧化物酶GSH-Px/(U/mg prot) 87.22±7.19b 47.04±4.75a 96.98±8.38b
总抗氧化能力T-AOC/(mmol/g prot) 0.06±0.01b 0.04±0.00a 0.08±0.00c
丙二醛MDA/(nmol/mg prot) 1.35±0.17a 1.95±0.10b 1.40±0.16a

2.4 大口黑鲈肝脏组织切片分析

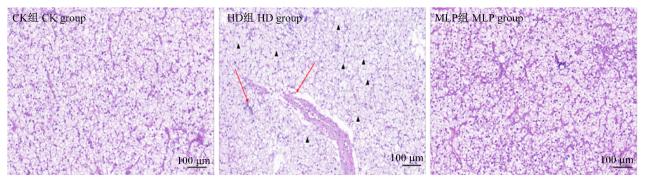
图1所示,CK组和MLP组大口黑鲈肝细胞排列紧密,细胞形态正常,组织未见明显坏死或炎症反应;而HD组肝细胞出现大量空泡化(三角形所示),偶见炎性细胞浸润(箭头所示)。
图1 大口黑鲈肝脏组织切片(HE染色)

三角形表示肝细胞空泡化,箭头表示炎性细胞浸润。

Fig.1 Liver tissue slices of Micropterus salmoides (HE staining)

Triangle indicated vacuolation of hepatocytes, and arrow indicated infiltration of inflammatory cells.

2.5 高淀粉饲料中添加MLP对大口黑鲈肝脏糖和脂代谢相关基因表达的影响

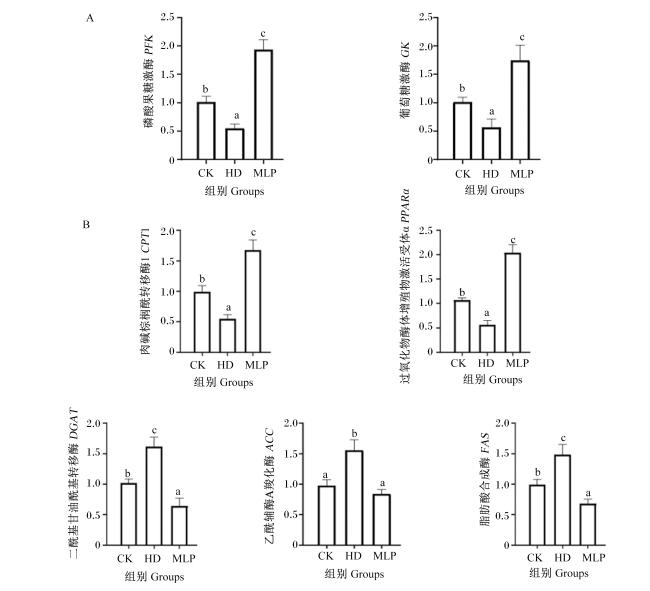
图2所示,与HD组相比,CK组和MLP组大口黑鲈肝脏PFKGKCPT1和PPARα mRNA相对表达量显著提高(P<0.05),肝脏DGATACCFAS mRNA相对表达量显著降低(P<0.05);与CK组相比,MLP组肝脏PFKGKCPT1和PPARα mRNA相对表达量显著提高(P<0.05),肝脏DGATFAS mRNA相对表达量显著降低(P<0.05)。
图2 高淀粉饲料中添加MLP对大口黑鲈肝脏糖和脂代谢相关基因表达的影响

A:糖代谢相关基因 genes related to glucose metabolism;B:脂代谢相关基因 genes related to lipid metabolism。

数据柱标注不同字母表示差异显著(P<0.05),无字母或相同字母表示差异不显著(P>0.05)。图3图5同。Value columns with different letters mean significant difference (P<0.05), while with the same letter or no letters mean no significant difference (P>0.05). The same as Fig.3 and Fig.5.

Fig.2 Effects of MLP supplementation in high starch diet on expression of genes related to liver glucose and lipid metabolism of Micropterus salmoides

2.6 高淀粉饲料中添加MLP对大口黑鲈肝脏炎症相关基因表达的影响

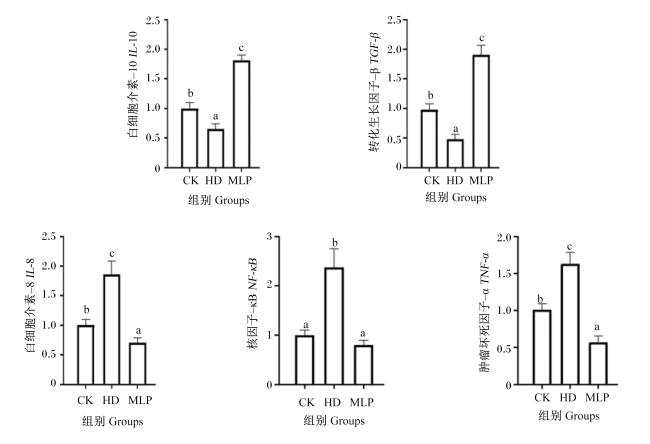
图3所示,与HD组相比,CK组和MLP组大口黑鲈肝脏IL-10和TGF-β mRNA相对表达量显著提高(P<0.05),肝脏IL-8、NF-κBTNF-α mRNA相对表达量显著降低(P<0.05);与CK组相比,MLP组肝脏IL-10和TGF-β mRNA相对表达量显著提高(P<0.05),肝脏IL-8和TNF-α mRNA相对表达量显著降低(P<0.05)。
图3 高淀粉饲料中添加MLP对大口黑鲈肝脏炎症相关基因表达的影响

Fig.3 Effects of MLP supplementation in high starch diet on expression of genes related to liver inflammation of Micropterus salmoides

2.7 高淀粉饲料中添加MLP对大口黑鲈肠道组织形态的影响

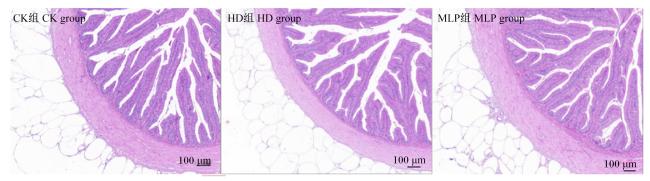
表6图4可知,各组大口黑鲈肠道结构完整。与HD组相比,CK组和MLP组肌层厚度显著增加(P<0.05);各组间肠绒毛高度和绒毛宽度无显著差异(P>0.05)。
表6 高淀粉饲料中添加MLP对大口黑鲈肠道组织形态的影响

Table 6 Effects of MLP supplementation in high starch diet on intestinal tissue morphology of Micropterus salmoides μm

项目
Items
组别Groups
CK HD MLP
绒毛高度Villus height 832.20±40.42 756.54±31.97 803.14±35.24
绒毛宽度Villus width 108.40±2.16 103.68±2.56 107.90±3.41
肌层厚度Thickness of muscular layer 196.82±6.49b 163.20±4.44a 186.64±5.37b
图4 大口黑鲈肠道组织切片(HE染色)

Fig.4 Intestinal tissue slices of Micropterus salmoides (HE staining)

2.8 高淀粉饲料中添加MLP对大口黑鲈肠道短链脂肪酸含量的影响

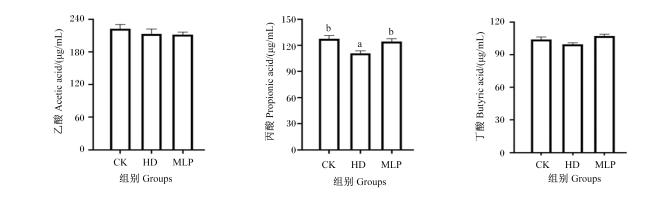
图5可知,与CK组相比,HD组大口黑鲈肠道丙酸含量显著降低(P<0.05),MLP组肠道丙酸含量无显著差异(P>0.05)。各组间肠道乙酸和丁酸含量均无显著差异(P>0.05)。
图5 高淀粉饲料中添加MLP对大口黑鲈肠道短链脂肪酸含量的影响

Fig.5 Effects of MLP supplementation in high starch diet on intestinal short-chain fatty acid contents of Micropterus salmoides

2.9 高淀粉饲料中添加MLP对大口黑鲈肠道菌群的影响

2.9.1 肠道菌群多样性

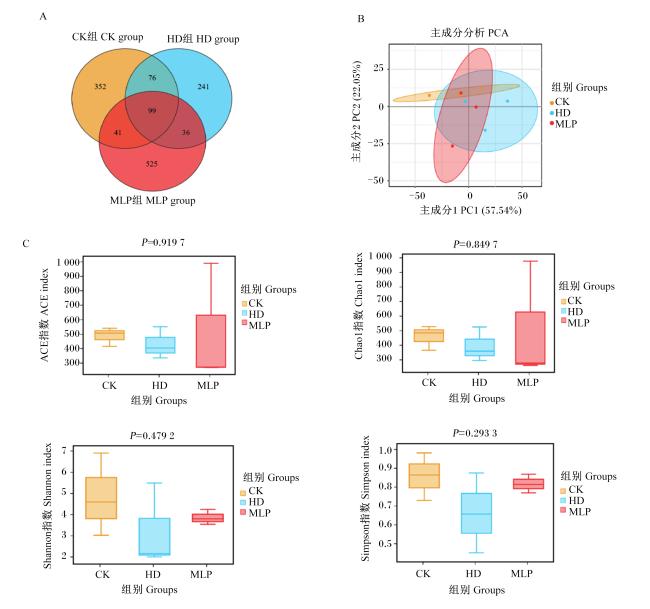
图6所示,3组大口黑鲈肠道菌群共检测到1 721个OTU,其中3组共有的OTU数目为99个,CK组、HD组和MLP组独有的OTU数目分别为352、241和525个。主成分分析(PCA)结果表明,CK组与HD组和MLP组聚类明显,且CK组和MLP组样品间距离更近,说明MLP组和CK组大口黑鲈肠道菌群组成更相似。各组间ACE指数、Chao1指数、Shannon指数和Simpson指数无显著差异(P>0.05)。
图6 高淀粉饲料中添加MLP对大口黑鲈肠道菌群多样性的影响

A:韦恩图 Venn chart;B:主成分分析 principal component analysis;C:α多样性 α diversity。

Fig.6 Effects of MLP supplementation in high starch diet on diversity of intestinal microbiota of Micropterus salmoides

2.9.2 肠道菌群组成

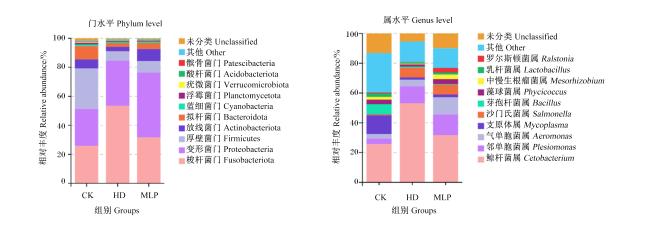
大口黑鲈肠道菌群在门和属水平上的组成如图7所示。在门水平上,优势菌群依次为梭杆菌门(Fusobacteriota)、变形菌门(Proteobacteria)、厚壁菌门(Firmicutes)、放线菌门(Actinobacteriota)和拟杆菌门(Bacteroidota),这5个菌门在各组肠道菌群中所占比例均在90%以上。与HD组相比,CK组和MLP组肠道拟杆菌门、放线菌门和厚壁菌门相对丰度升高(P>0.05),梭杆菌门相对丰度降低(P>0.05)。在属水平上,与HD组相比,CK组和MLP组肠道鲸杆菌属(Cetobacterium)相对丰度降低(P>0.05),乳杆菌属(Lactobacillus)相对丰度升高(P>0.05);MLP组气单胞菌属(Aeromonas)相对丰度升高(P>0.05)。
图7 高淀粉饲料中添加MLP对大口黑鲈肠道菌群组成的影响

Fig.7 Effects of MLP supplementation in high starch diet on intestinal microbiota composition of Micropterus salmoides

3 讨论

饲料中适宜的淀粉含量可以提高鱼类的生长性能,但添加量过高会损伤肠道,降低鱼体对营养物质的吸收能力。研究报道,饲喂高淀粉饲料会显著降低杂交鳢(Channa maculata♀×Channa argus♂)[17]、虹鳟(Oncorhynchus mykiss)[18]、珍珠龙胆石斑鱼(Epinephelus fuscoguttatus ♀×Epinephelus lanceolatus ♂)[19]和黄鳝(Monopterus albus)[20]的饲料利用率。在花鲈[21]和大口黑鲈[22]上的研究发现,投喂高淀粉饲料能促进摄食以维持自身的生长。本试验中,高淀粉饲料不改变大口黑鲈的FI和SGR,但显著降低了WGR,提高了FCR,添加MLP后WGR和FCR恢复到CK组水平,说明MLP可以提高大口黑鲈对饲料的利用率。Hao等[23]报道,豹纹鳃棘鲈(Plectropomus leopardus)饲料中添加黄芪多糖可以促进肠道组织发育,改善肠道菌群多样性和结构,从而显著提高其生长性能。高淀粉饲料中添加枸杞多糖能显著提高大口黑鲈肠道和肝脏消化酶活性,使其生长性能恢复甚至超过对照组[24]。研究表明,丁酸盐能改善受损黏膜细胞的修复,对于保持肠道上皮细胞的完整性和促进肠道发育至关重要[25]。类似地,本试验HD组肠道短链脂肪酸中的丙酸含量在添加MLP后显著升高,丁酸含量也呈上升趋势,同时肌层厚度显著增加,进而改善了肠道屏障,促进了营养物质的吸收。本试验结果表明,在高淀粉饲料中添加MLP可以显著提高鱼体对饲料的利用率,缓解高淀粉对大口黑鲈生长性能的负面影响。
当摄入过量的碳水化合物时,鱼体会将多余的GLU储存为GLY或脂质。血糖水平由肝脏通过糖异生和糖酵解等途径调控[26]。本试验中,高淀粉提高了血清TG和GLU以及肝脏TG和GLY含量,同时下调了肝脏PFK和GK的表达。PFK和PK是糖酵解途径中重要的限速酶。在本试验条件下,高淀粉饲料中添加MLP显著上调了肝脏PFKGK的表达,表明MLP可能通过促进丙酮酸的合成,从而加速糖类的氧化。同时,MLP通过刺激磷脂酰肌醇3-激酶(PI3K)-蛋白激酶B(AKT)信号通路,缓解胰岛素抵抗,显著降低了血糖含量[27]。本试验中,HD组肝脏GLY含量在添加MLP后显著降低,进一步表明MLP能促进肝糖原的分解。这与在黄鳝[20]和欧洲海鲈(Dicentrarchus labrax)[28]上的研究结果相似。研究表明,饲料中过高的淀粉含量会提高鱼类脂肪合成酶(如FAS和ACC)活性,促进脂质积蓄,导致肝脏肿大和HSI升高[29]。CPT1是参与脂肪分解代谢的关键酶之一,在PPARα的介导下,CPT1催化硫酰辅酶A转化为硫酰肉碱,从而启动线粒体中长链脂肪酸的β氧化;ACC催化乙酰辅酶A羧化为丙二酰辅酶A,随后FAS将之转化为棕榈酸,最终酯化为TG[30-31]。本研究结果表明,高淀粉饲料中添加MLP通过下调ACCFAS的表达,上调CPT1和PPARα的表达来抑制脂肪生成,加速脂肪酸氧化,从而降低了血清TG含量和肝脏的脂质沉积,这与MLP组大口黑鲈HSI显著降低的结果相一致。类似的结果在杂交鲶鱼(Pangasianodon gigas×Pangasianodon hypophthalmus)[32]和花鲈[33]上被证实。
研究表明,饲料中高碳水化合物压力超过机体的抗氧化能力时,肝脏会经历氧化应激,产生过量活性氧(ROS)和MDA,导致肝毒性和肝脏功能障碍,进而导致生理代谢紊乱[34-35]。肝脏的抗氧化系统[包括超氧化物歧化酶(superoxide dismutase,SOD)、过氧化氢酶(catalase,CAT)、GSH-Px、T-AOC和过氧化物酶(peroxidase,POD)等]在捕获和消除过量的ROS方面起着关键作用。Qi等[24]研究发现,枸杞多糖能显著提高饲喂高碳水化合物饲料大口黑鲈肠道和肝脏中SOD、CAT和GSH-Px活性及mRNA相对表达量,降低MDA含量。体外试验表明,MLP能剂量依赖性提高过氧化氢(H2O2)诱导的团头鲂(Megalobrama amblycephala)白细胞的抗氧化能力,有效缓解氧化损伤[36]。本研究中,饲喂高淀粉饲料显著降低了大口黑鲈肝脏T-AOC以及T-SOD和GSH-Px活性,显著提高了肝脏MDA含量,而添加MLP后显著提高了肝脏上述抗氧化酶的活性。这表明MLP能显著缓解高淀粉饲料造成的氧化应激和损伤,可能是MLP促进机体生成了谷氨酰胺、一氧化氮等物质,去除了各种组织细胞中的氧化物,从而减轻了对细胞的氧化损伤。
肝脏对免疫系统的贡献非常重要,免疫应激与抗氧化、炎症系统的激活密切相关[37-38]。IL-8作为一种炎性趋化因子,可趋化多种细胞至炎性组织;NF-κB和TNF-α是2种有效的促炎因子,可以通过调节其他细胞因子的表达来诱导炎症反应[39]。TGF-β和IL-10是多效性抗炎因子,通过抑制炎性细胞因子的释放来有效缓解炎症[40]。以往的研究表明,高碳水化合物饲料会引起TNF-α和白细胞介素-1β(IL-1β)基因表达的显著上调,从而诱导炎症反应[41-42]。植物多糖具有免疫双向调节作用,即在正常生理条件下,可以通过促进细胞因子的产生来增强机体的免疫力;而在炎症发生后,可以减少促炎细胞因子的表达并保护细胞[43]。本试验中,HD组大口黑鲈肝脏中免疫相关基因IL-8、NF-κBTNF-α表达显著上调,肝脏IL-10和TGF-β表达显著下调,在添加MLP后其表达量表现出相反的结果,这表明在高淀粉饲料中添加MLP显著缓解了大口黑鲈肝脏的炎症反应,保护肝脏免受氧化应激损伤。血液中ALT和AST的活性是诊断肝脏损伤的重要指标。Zhou等[44]研究报道,不添加淀粉或者高淀粉供应均会导致金鲳鱼(Trachinotus ovatus)幼鱼血浆AST和ALT活性的升高,免疫能力的降低,从而导致幼鱼死亡率升高。高碳水饲料会导致乌鳢(Channa argus)内质网应激,并伴随着细胞自噬以及血清AST和ALT活性的升高[45]。本试验中,高淀粉导致大口黑鲈血清AST和ALT活性的显著升高,肝细胞空泡化加剧;而添加MLP后血清AST和ALT活性以及肝细胞空泡化数目显著降低。本试验血清生化指标和肝脏组织切片分析的结果进一步表明MLP能缓解高淀粉导致的肝脏炎症和肝脏损伤,提高大口黑鲈的免疫能力。
碳水化合物可通过调节肠道微生物群落来影响肠道健康和肠道功能。研究表明,饲料中添加5%~20%的玉米淀粉会提高卵形鲳鲹肠道弧菌属(Vibrio)、发光杆菌属(Photobacterium)和支原体属(Mycoplasma)等致病菌的相对丰度,提高卵形鲳鲹患病概率[46]。Zhang等[29]报道,高淀粉会降低鳜鱼肠道产丁酸菌(厚壁菌门、拟杆菌门)的相对丰度,增加肠道脂滴的积聚,导致肠道通透性增加,最终导致肠道炎症。植物多糖在抑制有害菌增殖的同时,增加有益菌的数量,促进短链脂肪酸的生成[47]。类似地,本研究中,HD组肠道厚壁菌门、拟杆菌门相对丰度和丁酸含量低于CK组;而添加MLP后厚壁菌门和拟杆菌门相对丰度升高,丁酸含量也呈上升趋势。丁酸能刺激机体产生细胞免疫和体液免疫反应,说明高淀粉饲料中添加MLP能提高大口黑鲈的免疫和抗病能力。厚壁菌门中的乳杆菌属可显著提高鱼肠道消化酶活性,并参与体内碳水化合物的发酵[48]。本研究发现,MLP组肠道乳杆菌属相对丰度高于HD组,说明高淀粉饲料中添加MLP能增强大口黑鲈的消化吸收能力,这可能是该组生长性能显著提升并与CK组持平的原因之一。肠道菌群的α多样性分析可以反映微生物群落的丰富度和和多样性。本研究发现,相比于HD组,MLP组Simpson指数和Shannon指数呈现上升趋势,这与黄芪多糖在克氏原鳌虾(Procambarus clarkii)[49]、浒苔多糖在花鲈[50]上的研究结果类似,说明MLP能有效恢复高淀粉胁迫下肠道菌群的多样性,从而维持大口黑鲈肠道健康。

4 结论

高淀粉饲料诱导了氧化应激和炎症反应,造成糖、脂代谢和肠道菌群紊乱,导致大口黑鲈生长性能降低。在高淀粉饲料中添加MLP可以提高大口黑鲈生长性能、抗氧化能力、肠道菌群多样性和有益菌相对丰度,缓解肝脏炎症,并通过加速糖类和脂肪酸氧化,抑制胰岛素抵抗,促进糖和脂代谢。
[1]
LIU Q Q, XIA R, DENG X, et al. Effects of dietary starch and metformin levels on the growth performance,body composition,hepatic glycolipid metabolism,and liver histology of juvenile largemouth bass Micropterus salmoides[J]. Aquaculture, 2023, 573:739582.

DOI

[2]
LI X Y, ZHENG S X, MA X K, et al. Effects of dietary starch and lipid levels on the protein retention and growth of largemouth bass (Micropterus salmoides)[J]. Amino Acids, 2020, 52(6/7):999-1016.

DOI

[3]
ZHANG Y M, XIE S W, WEI H L, et al. High dietary starch impaired growth performance,liver histology and hepatic glucose metabolism of juvenile largemouth bass,Micropterus salmoides[J]. Aquaculture Nutrition, 2020, 26(4):1083-1095.

DOI

[4]
ZHOU Y L, HE G L, JIN T, et al. High dietary starch impairs intestinal health and microbiota of largemouth bass,Micropterus salmoides[J]. Aquaculture, 2021, 534:736261.

DOI

[5]
缪子敬, 李志万, 周学海, 等. α-葡萄糖苷酶抑制剂的研究进展[J]. 广东化工, 2019, 46(17):96-97,101.

MIU Z J, LI Z W, ZHOU X H, et al. Research progress of α-glucosidase inhibitors[J]. Guangdong Chemical Industry, 2019, 46(17):96-97,101. (in Chinese)

[6]
CHEN R H, ZHOU X, DENG Q F, et al. Extraction,structural characterization and biological activities of polysaccharides from mulberry leaves:a review[J]. International Journal of Biological Macromolecules, 2024, 257(Pt 2):128669.

DOI

[7]
ZHANG Y, REN C J, LU G B, et al. Anti-diabetic effect of mulberry leaf polysaccharide by inhibiting pancreatic islet cell apoptosis and ameliorating insulin secretory capacity in diabetic rats[J]. International Immunopharmacology, 2014, 22(1):248-257.

DOI PMID

[8]
陈晓兰, 宣嘉颖, 王婧, 等. 桑叶多糖对免疫抑制小鼠肠道损伤和微生物多样性的调节作用[J]. 动物营养学报, 2022, 34(3):1996-2008.

DOI

CHEN X L, XUAN J Y, WANG J, et al. Regulating effects of mulberry leaf polysaccharide on intestinal damage and microbial diversity of immunosuppressed mice[J]. Chinese Journal of Animal Nutrition, 2022, 34(3):1996-2008. (in Chinese)

[9]
LI H T, LU L, WU M, et al. The effects of dietary extract of mulberry leaf on growth performance,hypoxia-reoxygenation stress and biochemical parameters in various organs of fish[J]. Aquaculture Reports, 2020, 18:100494.

DOI

[10]
ZHOU S S, HUANG Z F, LIN H, et al. Effects of mulberry leaf extract on the intestinal health of spotted sea bass (Lateolabrax maculatus)[J]. Frontiers in Marine Science, 2023, 10:1185795.

DOI

[11]
ZHOU S S, LIN H, KONG L M, et al. Effects of mulberry leaf extract on the liver function of juvenile spotted sea bass (Lateolabrax maculatus)[J]. Aquaculture Nutrition, 2023, 2023:2892463.

[12]
周东来, 刘凡, 汪福保, 等. 桑叶提取物对鳜鱼生长性能、血清免疫指标、抗氧化能力及肝脏和肠道健康的影响[J]. 动物营养学报, 2023, 35(2):1147-1159.

DOI

ZHOU D L, LIU F, WANG F B, et al. Effects of mulberry leaf extract on growth performance,serum immune indices,antioxidant ability and liver and intestinal health of Siniperca chuatsi[J]. Chinese Journal of Animal Nutrition, 2023, 35(2):1147-1159. (in Chinese)

[13]
符兵, 彭凯, 陈冰, 等. 饲料中添加蚕豆对罗非鱼生长性能、肠道消化酶活性、肠道形态和肠道菌群的影响[J]. 动物营养学报, 2023, 35(1):494-504.

DOI

FU B, PENG K, CHEN B, et al. Effects of Faba bean supplementation on growth performance,intestinal digestive enzyme activities,intestinal morphology and intestinal flora of tilapia (Oreochromis niloticus)[J]. Chinese Journal of Animal Nutrition, 2023, 35(1):494-504. (in Chinese)

[14]
HU T G, YU Y S, WU J J, et al. Structural elucidation of mulberry leaf oligosaccharide and its selective promotion of gut microbiota to alleviate type 2 diabetes mellitus[J]. Food Science and Human Wellness, 2024, 13(4):2161-2173.

DOI

[15]
CAPORASO J G, KUCZYNSKI J, STOMBAUGH J, et al. QIIME allows analysis of high-throughput community sequencing data[J]. Nature Methods, 2010, 7(5):335-336.

DOI PMID

[16]
LIVAK K J, SCHMITTGEN T D. Analysis of relative gene expression data using real-time quantitative PCR and the 2-ΔΔCT method[J]. Methods, 2001, 25(4):402-408.

DOI

[17]
李培佳, 吕旦, 李敏, 等. 高碳水化合物饲料添加牛磺酸对杂交鳢生长性能、肝脏糖代谢相关基因表达、抗氧化活性及免疫应答的影响[J]. 动物营养学报, 2023, 35(11):7320-7334.

DOI

LI P J, LYU D, LI M, et al. Effects of taurine supplementation in high carbohydrate diet on growth performance,gene expression related to liver glucose metabolism,and antioxidant activity and immune response of hybrid snakehead [Channa maculata (♀)×C. argus (♂)][J]. Chinese Journal of Animal Nutrition, 2023, 35(11):7320-7334. (in Chinese)

[18]
ZHAO W, WEI H L, WANG Z Q, et al. Effects of dietary carbohydrate levels on growth performance,body composition,antioxidant capacity,immunity,and liver morphology in Oncorhynchus mykiss under cage culture with flowing freshwater[J]. Aquaculture Nutrition, 2022, 2022:7820017.

[19]
LI S L, LI Z Q, ZHANG J C, et al. The impacts of dietary carbohydrate levels on growth performance,feed utilization,glycogen accumulation and hepatic glucose metabolism in hybrid grouper (Epinephelus fuscoguttatus ♀×E. lanceolatus ♂)[J]. Aquaculture, 2019, 512:734351.

DOI

[20]
SHI Y, ZHONG L, FAN Y D, et al. The protective effect of mulberry leaf flavonoids on high-carbohydrate-induced liver oxidative stress,inflammatory response and intestinal microbiota disturbance in Monopterus albus[J]. Antioxidants, 2022, 11(5):976.

DOI

[21]
孙文豪, 邱建强, 田仁红, 等. 高糖饲料及添加缩合单宁对花鲈生长性能、体成分、血清代谢物、肠道短链脂肪酸含量及激素基因表达的影响[J]. 动物营养学报, 2024, 36(8):5254-5268.

DOI

SUN W H, QIU J Q, TIAN R H, et al. Effects of high sugar diet and condensed tannin supplementation on growth performance,body composition,serum metabolites,intestinal short-chain fatty acid contents and hormone gene expression of sea bass (Lateolabrax maculatus)[J]. Chinese Journal of Animal Nutrition, 2024, 36(8):5254-5268. (in Chinese)

[22]
LIN S M, SHI C M, MU M M, et al. Effect of high dietary starch levels on growth,hepatic glucose metabolism,oxidative status and immune response of juvenile largemouth bass,Micropterus salmoides[J]. Fish & Shellfish Immunology, 2018, 78:121-126.

[23]
HAO X Q, LIN H Z, LIN Z Y, et al. Effect of dietary Astragalus polysaccharides (APS) on the growth performance,antioxidant responses,immunological parameters,and intestinal microbiota of coral trout (Plectropomus leopardus)[J]. Microorganisms, 2024, 12(10):1980.

DOI

[24]
QI L, HE Y Y, ZHONG G F. Dietary Lycium barbarum polysaccharide modulates growth performance,antioxidant capacity,and glucolipid metabolism in largemouth bass (Micropterus salmoides) fed with high-carbohydrate diet[J]. Frontiers in Marine Science, 2025, 12:1542173.

DOI

[25]
李祥, 何金环, 潘春梅, 等. 丁酸钠对鱼类肠道消化吸收的影响研究进展[J]. 中国畜牧兽医, 2022, 49(1):131-139.

DOI

LI X, HE J H, PAN C M, et al. Research progress on effects of sodium butyrate on intestinal digestion and absorption of fish[J]. China Animal Husbandry & Veterinary Medicine, 2022, 49(1):131-139. (in Chinese)

[26]
POLAKOF S, PANSERAT S, SOENGAS J L, et al. Glucose metabolism in fish:a review[J]. Journal of Comparative Physiology B, 2012, 182(8):1015-1045.

DOI

[27]
REN C J, ZHANG Y, CUI W Z, et al. A polysaccharide extract of mulberry leaf ameliorates hepatic glucose metabolism and insulin signaling in rats with type 2 diabetes induced by high fat-diet and streptozotocin[J]. International Journal of Biological Macromolecules, 2015, 72:951-959.

PMID

[28]
TORRECILLAS S, MONTERO D, CABALLERO M J, et al. Effects of dietary concentrated mannan oligosaccharides supplementation on growth,gut mucosal immune system and liver lipid metabolism of European sea bass (Dicentrarchus labrax) juveniles[J]. Fish & Shellfish Immunology, 2015, 42(2):508-516.

[29]
ZHANG Y P, LIANG X F, HE S, et al. Effects of high carbohydrate diet-modulated microbiota on gut health in Chinese perch[J]. Frontiers in Microbiology, 2020, 11:575102.

DOI

[30]
TORRÓ-MONTELL L, CORTÉS-CASTELL E, SIRVENT-SEGURA E, et al. Influence of olive extracts on the expression of genes involved in lipid metabolism in medaka fish[J]. Molecules, 2019, 24(17):3068.

DOI

[31]
HUANG D Y, LIANG H L, REN M C, et al. Effects of dietary lysine levels on growth performance,whole body composition and gene expression related to glycometabolism and lipid metabolism in grass carp,Ctenopharyngodon idellus fry[J]. Aquaculture, 2021, 530:735806.

DOI

[32]
HAHOR W, THONGPRAJUKAEW K, SUANYUK N. Effects of dietary supplementation of oligosaccharides on growth performance,gut health and immune response of hybrid catfish (Pangasianodon gigas×Pangasianodon hypophthalmus)[J]. Aquaculture, 2019, 507:97-107.

DOI

[33]
HUANG Z F, YE Y L, LONG Z Y, et al. Lycium barbarum polysaccharides improve lipid metabolism disorders of spotted sea bass Lateolabrax maculatus induced by high lipid diet[J]. International Journal of Biological Macromolecules, 2023, 242(Pt 3):125122.

DOI

[34]
MA H J, MOU M M, PU D C, et al. Effect of dietary starch level on growth,metabolism enzyme and oxidative status of juvenile largemouth bass,Micropterus salmoides[J]. Aquaculture, 2019, 498:482-487.

DOI

[35]
ZHENG L Z, WANG Z Z, ZHANG B, et al. Effects of high dietary carbohydrate levels on growth performance,enzyme activities,expression of genes related to liver glucose metabolism,and the intestinal microbiota of Lateolabrax maculatus juveniles[J]. Fishes, 2023, 8(9):431.

DOI

[36]
JIANG W Q, LIN Y, QIAN L J, et al. Mulberry leaf polysaccharides attenuate oxidative stress injury in peripheral blood leukocytes by regulating endoplasmic reticulum stress[J]. Antioxidants, 2024, 13(2):136.

DOI

[37]
YU Z, ZHAO Y Y, JIANG N, et al. Bioflocs attenuates lipopolysaccharide-induced inflammation,immunosuppression and oxidative stress in Channa argus[J]. Fish & Shellfish Immunology, 2021, 114:218-228.

[38]
NIU X T, SUN C, ZHAO L, et al. The major role of glucocorticoid receptor (GR) in astaxanthin alleviates immune stress in Channa argus lymphocyte[J]. Aquaculture, 2024, 584:740637.

DOI

[39]
KONG Y D, LI M, GUO G L, et al. Effects of dietary curcumin inhibit deltamethrin-induced oxidative stress,inflammation and cell apoptosis in Channa argus via Nrf2 and NF-κB signaling pathways[J]. Aquaculture, 2021, 540:736744.

DOI

[40]
LI K, LI J Q, WEI X M, et al. IL-10 negatively controls the primary T cell response of tilapia by triggering the JAK1/STAT3/SOCS3 axis that suppresses NF-κB and MAPK/ERK signaling[J]. The Journal of Immunology, 2023, 210(3):229-244.

DOI

[41]
CHEN P, ZHU Y P, WU X F, et al. Metabolic adaptation to high starch diet in largemouth bass (Micropterus salmoides) was associated with the restoration of metabolic functions via inflammation,bile acid synthesis and energy metabolism[J]. British Journal of Nutrition, 2022, 129(3):381-394.

DOI

[42]
WANG K W, LIU Q Q, ZHU J, et al. Transcriptome analysis provides insights into the molecular mechanism of liver inflammation and apoptosis in juvenile largemouth bass Micropterus salmoides fed low protein high starch diets[J]. Comparative Biochemistry and Physiology Part D:Genomics and Proteomics, 2023, 45:101047.

DOI

[43]
ZHENG Y J, REN W Y, ZHANG L N, et al. A review of the pharmacological action of Astragalus polysaccharide[J]. Frontiers in Pharmacology, 2020, 11:349.

DOI

[44]
ZHOU C P, GE X P, LIN H Z, et al. Effect of dietary carbohydrate on non-specific immune response,hepatic antioxidative abilities and disease resistance of juvenile golden pompano (Trachinotus ovatus)[J]. Fish & Shellfish Immunology, 2014, 41(2):183-190.

[45]
LI M Y, LIU Y Z, CHEN X M, et al. Astaxanthin ameliorates high-carbohydrate diet-induced ER stress,immunosuppression and hepatic glucose metabolism through AMPK/autophagy pathway in Channa argus[J]. Aquaculture, 2025, 598:742010.

DOI

[46]
ZHAO W, XIE J J, FANG H H, et al. Effects of corn starch level on growth performance, antioxidant capacity,gut morphology and intestinal microflora of juvenile golden pompano,Trachinotus ovatus[J]. Aquaculture, 2020, 524:735197.

DOI

[47]
SHI F, LU Z J, YANG M X, et al. Astragalus polysaccharides mediate the immune response and intestinal microbiota in grass carp (Ctenopharyngodon idellus)[J]. Aquaculture, 2021, 534:736205.

DOI

[48]
VALIALLAHI J, POURABASALI M, JANALIZADEH E, et al. Use of Lactobacillus for improved growth and enhanced biochemical,hematological,and digestive enzyme activity in common carp at Mazandaran,Iran[J]. North American Journal of Aquaculture, 2018, 80(2):206-215.

DOI

[49]
PEI Q L, HE M X, TANG P, et al. Salvia miltiorrhiza polysaccharide promotes the health of crayfish (Procambarus clarkii) by promoting hemocyte phagocytosis,protecting hepatopancreas and enhancing intestinal barrier function[J]. Fish & Shellfish Immunology, 2024, 146:109405.

[50]
LONG Z Y, LIU L H, QIN H H, et al. Effects of Enteromorpha prolifera polysaccharide on intestinal health of spotted sea bass Lateolabrax maculatus[J]. Aquaculture Reports, 2025, 40:102584.

DOI

Outlines

/