RESEARCH PAPER

Effects of Codonopsis pilosula Polysaccharides on Growth Performance, Nutrient Digestion, Rumen Fermentation and Microbiota in Yak Calves

  • CHENG Wenbo , 1, 2 ,
  • CIDAN Yangji 2 ,
  • CISANG Zhuoma 2 ,
  • GUSANG Deji 2 ,
  • DEJI Quzhen 2 ,
  • BASANG Wangdui 2 ,
  • XING Yahui 1 ,
  • HAN Chengxing 1 ,
  • GUO Yanli , 1, * ,
  • ZHU Yanbin , 2, *
Expand
  • 1 College of Animal Science and Technology, Gansu Agricultural University, Lanzhou 730070, China
  • 2 Xizang Academy of Agriculture and Animal Husbandry Sciences, Lhasa 850000, China
* GUO Yanli, professor, E-mail: ;
ZHU Yanbin, professor, E-mail:

Received date: 2025-06-27

  Online published: 2026-01-13

Abstract

The aim of this experiment was to investigate the effects of Codonopsis pilosula polysaccharides (CPP) on growth performance, nutrient digestion, rumen fermentation and microbiota in yak calves. A one-way randomized experimental design was used to select 27 yak male calves around 6 months of age, with an average weight of (72.61±1.35) kg and in good health condition, and randomly divided into three groups: control group (CN group, fed only the basal diet), low-dose group (DSL group, with 5 g/d of CPP added to the basal diet), and high-dose group (DSH group, with 10 g/d of CPP added to the basal diet). Nine replicates of 1 cow per group were housed in a single pen. The pre-test period was 10 d, and the positive test period was 60 d. Results showed as follows: 1) the average daily gain (ADG) of the DSH group was extremely significantly higher than that of the CN group (P<0.01), the final body weight (FBW) and average daily feed intake (ADFI) were significantly higher than that of the CN group (P<0.05), and the ADFI was significantly higher than that of the DSL group (P<0.05). 2) The neutral detergent fiber (NDF) digestibility of the DSH group was significantly higher than that of the CN group and DSL group (P<0.05). 3) The total volatile fatty acid (TVFA) concentration of the DSH group was extremely significantly higher than that of the CN group and DSL group (P<0.01), and the acetic acid (AA) concentration was significantly higher than that of the CN group and DSL group (P<0.05) 4) The Shannon index, ACE index, and Chao1 index of the DSH group were extremely significantly higher than those of the CN group (P<0.01), the ACE index and Chao1 index of the DSL group were extremely significantly higher than those of the CN group (P<0.01), and the ACE index of the DSH group was extremely significantly higher than that of the DSL group (P<0.01); at the rumen microbial genus level, the relative abundance of Ruminococcus in the DSH group was extremely significantly higher than that of the CN group (P<0.01), and the relative abundance of Candidatus_Saccharimonas was significantly higher than that of the CN group (P<0.05); functional prediction analysis results showed that the lipid metabolism, folding, sorting and degradation pathways were extremely significantly enriched in the DSH group (P<0.01), and the coenzyme and vitamin metabolism, terpenoid and polyketide metabolism pathways were significantly enriched in the DSH group (P<0.05). 5) Correlation analysis showed that ADG, ADFI, concentrations of TVFA and AA were significantly positively correlated with the relative abundance of Ruminococcus and the coenzyme and vitamin metabolism pathway (P<0.05); ADFI, concentrations of TVFA and AA were significantly positively correlated with the folding, sorting and degradation pathway (P<0.05); F/G was significantly positively correlated with other amino acid metabolism pathway (P<0.05). The above results indicate that the addition of CPP to the diet can improve growth performance, NDF digestibility, TVFA and AA concentrations, and rumen microflora in yak calves.

Cite this article

CHENG Wenbo , CIDAN Yangji , CISANG Zhuoma , GUSANG Deji , DEJI Quzhen , BASANG Wangdui , XING Yahui , HAN Chengxing , GUO Yanli , ZHU Yanbin . Effects of Codonopsis pilosula Polysaccharides on Growth Performance, Nutrient Digestion, Rumen Fermentation and Microbiota in Yak Calves[J]. Chinese Journal of Animal Nutrition, 2026 , 38(1) : 442 -455 . DOI: 10.12418/CJAN2026.035

牦牛是生活于青藏高原及其周边高山和亚高山区域的特殊牛种,这种特殊的地理地貌使它对少氧、寒冷环境有着良好的适应性[1]。然而,由于生长速度缓慢、饲料转化率低等问题限制了其生产性能和经济效益的提升,探索有效的营养策略以改善牦牛犊牛的生长发育非常重要。瘤胃作为反刍动物独特的消化器官,是最高效的生物反应器,瘤胃微生物的降解和发酵可以提高瘤胃的消化吸收能力和营养物质的新陈代谢,在反刍动物营养中起着重要作用[2]
党参为桔梗科植物,其植物化学成分复杂,含有多糖类、黄酮类、萜类等多种成分[3],在我国西北、华北和东北地区分布广泛。其中,西北地区因独特的地理优势和自然条件,为党参的生长提供了良好的环境,它的种植面积高达75.7万亩(1亩≈0.066 7 hm2),产量约占全国的60%[4]。党参多糖(CPP)是党参药材中重要的活性成分,含量达10%~20%[5],具有抗肿瘤[6]、抗衰老[7]、免疫调节[8]等多种生物学作用。隋奉桐等[9]研究发现,在断奶仔猪饲粮中加入400和800 mg/kg的CPP可使仔猪的终末体重(FBW)、平均日增重(ADG)显著提高并降低料重比(F/G),并且不同添加量的CPP也在一定程度上增加了免疫球蛋白的含量。Tang等[10]在小鼠饲粮中添加300和600 mg/kg的CPP发现,试验组厚壁菌门和拟杆菌门的相对丰度提高,小鼠肠道微生物结构得到改善,且小鼠的体重增长率显著高于模型组。此外,孙嘉琪[11]使用CPP灌胃急性氧化损伤小鼠后发现,CPP不仅能显著提高小鼠体重,还可有效缓解过氧化氢诱导下的免疫应激,提高血清中超氧化物歧化酶(SOD)及谷胱甘肽过氧化酶(GSH-Px)的活性,降低活性氧(ROS)的含量,进而增强机体抗氧化能力。Zhang等[12]研究发现,CPP可刺激小鼠巨噬细胞的增殖,还能显著提高肿瘤坏死因子-α(TNF-α)的分泌和淋巴细胞内CD4+含量,且CD4+与CD8+的比例也趋向于正常范围,增强了小鼠的特异性和非特异性免疫。还有研究发现,CPP可通过促进肠道有益菌的生长,同时抑制有害菌的生长来维持微生物区系间的平衡,进而促进乙酸(AA)浓度增加,表明CPP可维持肠道内环境稳定,同时又提高了厚壁菌门和拟杆菌门的比例,改善了肠道微生物生态失调[13]
CPP已在小鼠等模式动物中被证明具有促进生长、免疫调节、抗氧化及调节肠道微生物区系等多种生理功能,但在反刍动物尤其是牦牛中的研究较少。因此,本研究以牦牛犊牛为研究对象,探究CPP对其生长性能、养分消化、瘤胃发酵和微生物区系的影响,为牦牛生产中饲料添加剂的开发应用提供科学依据。

1 材料与方法

1.1 伦理声明

本研究使用的试验动物和试验设计方案已获得西藏农科院实验动物伦理委员会的批准(审批编号:TAAHS-2023-62)。

1.2 试验材料

CPP(纯度≥98%)购自于上海某生物科技有限公司;牦牛犊牛由西藏林周县格桑塘现代农牧产业示范园提供。

1.3 试验设计与饲粮

试验采用单因子随机试验设计,选取月龄(6月龄左右)、体重[(72.61±1.35) kg]相近且健康状况良好的牦牛公犊27头,随机分为3组:对照组(CN组,仅饲喂基础饲粮)、低剂量组(DSL组,在基础饲粮中添加5 g/d的CPP)和高剂量组(DSH组,在基础饲粮中添加10 g/d的CPP),每组9个重复,每个重复1头牛。CPP的添加剂量根据Tang等[10]在小鼠上的试验结果,经体重换算得到。试验共进行70 d,其中预试期10 d,正试期60 d。所有试验犊牛采取单栏舍饲,基础饲粮参照《肉牛饲养标准》(NY/T 815—2004)配制,其组成及营养水平如表1所示。CPP每天在饲喂前直接混合在颗粒料中饲喂。
表1 基础饲粮组成及营养水平(干物质基础)

Table 1 Composition and nutrient levels of the basal diet (DM basis) %

项目Items 含量Content
原料Ingredients
小麦秸秆Wheat straw 40.00
苜蓿干草Alfalfa hay 20.00
玉米Corn 20.00
豆粕Soybean meal 10.00
麸皮Wheat bran 5.00
膨化大豆Puffed soybean 2.00
食盐NaCl 0.50
碳酸氢钙Ca(HCO3)2 0.50
预混料Premix1) 2.00
合计Total 100.00
营养水平Nutrient levels2)
粗蛋白质CP 13.86
粗灰分Ash 8.47
中性洗涤纤维NDF 34.19
酸性洗涤纤维ADF 19.61
钙Ca 0.36
磷P 0.31
代谢能ME/(MJ/kg) 6.48

1)预混料为每千克饲粮提供 The premix provided the following per kg of the basal diet:VA 14 000 IU,VD3 2 800 IU,VE 40 IU,Cu 15 mg,Fe 50 mg,Zn 30 mg,Mn 50 mg,Se 0.4 mg,I 0.9 mg,Co 0.4 mg。

2)代谢能为计算值,根据《肉牛饲养标准》(NY/T 815—2004)计算,其余均为实测值。ME was a calculated value, according to Standards for Raising Beef Cattle (NY/T 815—2004), while the others were measured values.

1.4 饲养管理

本试验于2024年7—10月,在西藏林周县格桑塘现代农牧产业示范园(北纬29°5″,东经91°11″)进行。养殖场海拔3 870 m左右,试验期牛舍温度为8~20 ℃。试验开始前对圈舍进行清扫和消毒,预试期间对牛只体内驱虫并记录耳号。每天分别于09:00和17:00各饲喂1次,先粗后精,自由采食和饮水,定期对圈舍进行消毒。试验期间每天观察牛只采食、反刍及粪便情况,未发现异常。

1.5 测定指标及方法

1.5.1 生长性能

分别于正试期第1、60天对试验牛进行空腹称重,记录初始体重(IBW)和FBW,计算ADG,并记录采食量。每次饲喂时准确记录投料量,次日清晨称剩料量,计算平均日采食量(ADFI)和F/G。
ADG=(FBW-IBW)/试验天数;
ADFI=[(投料量-剩料量)×饲粮干物质(DM)含量]/试验天数;
F/G=ADFI/ADG。

1.5.2 养分消化率

正试期每周收集1次饲粮样品,并制成风干样进行保存。试验结束前7 d采用内源指示剂法进行消化试验,采集所有牛只(27头)每日清晨的粪便样品分为2份,其中一份加入10%硫酸固氮,另一份不做处理,将2份放入-20 ℃冰箱保存,再将采集到的粪样充分混合后,使用“四分法”取样,烘干粉碎后装入自封袋中保存备测。
饲粮DM、粗蛋白质(CP)、中性洗涤纤维(NDF)、酸性洗涤纤维(ADF)、钙(Ca)和磷(P)含量分别参照GB/T 6435—2014、GB/T 6432—2018、GB/T 20806—2022、NY/T 1459—2022和GB/T 13885—2017中方法进行测定。采用酸不溶灰分(AIA)法测定养分消化率[14],计算公式如下:
某养分消化率(%)=100-[(饲粮中AIA含量×粪中该养分含量)/(粪中AIA含量×饲粮中该养分含量)]×100。

1.5.3 瘤胃发酵参数

所有犊牛在试验最后1 d晨饲前,采用口腔插管法采集瘤胃液,将消毒好的瘤胃导管插入瘤胃内,为防止唾液污染,用注射器缓慢抽取50 mL瘤胃液后弃去不用,再次采集50 mL瘤胃液并用4层灭菌纱布过滤后分装于5 mL冻存管内,立即投入液氮罐中,带回实验室-80 ℃保存,用于测定瘤胃发酵参数。瘤胃液中氨态氮(NH3-N)浓度参照冯宗慈等[15]的比色法进行测定,挥发性脂肪酸浓度参照Li等[16]的方法,采用气相色谱仪(安捷伦7890B,美国)进行测定。

1.5.4 瘤胃微生物区系

将瘤胃液样品在干冰条件下送至上海美吉生物医药科技有限公司进行16S rRNA基因测序分析。使用Nanodrop测定DNA浓度和纯度,并通过琼脂糖凝胶电泳检测DNA完整性。从各组犊牛的瘤胃内容物中提取总DNA,然后使用通用引物338F(5'-ACTCCTACGGGAGGCAGCAG-3')和806R(5'-GGACTACHVGGGTWTCTAAT-3')对细菌16S rRNA基因的V3~V4可变区进行聚合酶链式反应(PCR)扩增。PCR扩增条件为95 ℃预变性3 min;95 ℃变性30 s,55 ℃退火30 s,72 ℃延伸45 s,共30个循环;72 ℃延伸10 min。PCR扩增产物使用1.0%琼脂糖凝胶电泳检测,使用Agencourt AMPure XP核酸纯化试剂盒(Beckman Coulter公司)进行自动化纯化,文库在Illumina NovaSeq平台进行双端测序(PE250),单个样本测序数据量≥5 000 reads以确保稀有物种检出效能。Alpha多样性包括了Shannon指数、Simpson指数、ACE指数和Chao1指数,以评估微生物丰富度和均匀度。Beta多样性基于Bray-Curtis距离进行主坐标分析(PCoA),评估组间微生物区系结构差异。

1.6 数据统计分析

采用Excel 2021进行数据的初步处理,利用SPSS 26.0统计软件进行one-way ANOVA方差分析,差异显著时用Duncan氏法进行多重比较,结果用平均值和均值标准误(SEM)表示,P<0.01表示差异极显著,P<0.05表示差异显著。

2 结果与分析

2.1 CPP对牦牛犊牛生长性能的影响

表2可知,DSH组犊牛ADG极显著高于CN组(P<0.01),FBW和ADFI显著高于CN组(P<0.05),并且DSH组犊牛ADFI显著高于DSL组(P<0.05),2个添加剂量组的FBW、ADG无显著差异(P≥0.05)。其余指标在各组间无显著差异(P≥0.05)。
表2 CPP对牦牛犊牛生长性能的影响

Table 2 Effects of CPP on growth performance of yak calves

项目
Items
组别Groups SEM P
P-value
CN DSL DSH
初始体重IBW/kg 70.93 72.93 73.93 1.155 0.582
终末体重FBW/kg 100.36b 105.07ab 111.79a 1.875 0.034
平均日增重ADG/(g/d) 490.48Bb 535.71ABab 630.95Aa 20.543 0.009
平均日采食量ADFI/(kg/d) 5.34b 5.66b 6.87a 0.265 0.012
料重比F/G 11.81 12.04 10.85 0.477 0.623

同行数据肩标无字母或相同字母表示差异不显著(P≥0.05),不同小写字母表示差异显著(P<0.05),不同大写字母表示差异极显著(P<0.01)。下表同。

In the same row, values with no letter or the same letter superscripts mean no significant difference (P≥0.05), while with different small letter superscripts mean significant difference (P<0.05), and with different capital letter superscripts mean extremely significant difference (P<0.01). The same as below.

2.2 CPP对牦牛犊牛养分消化率的影响

表3可知,DSH组NDF消化率显著高于CN组和DSL组(P<0.05),DSL组与CN组的NDF消化率无显著差异(P≥0.05)。其余指标在各组间无显著差异(P≥0.05)。
表3 CPP对牦牛犊牛养分消化率的影响

Table 3 Effects of CPP on nutrient digestibility of yak calves %

项目
Items
组别Groups SEM P
P-value
CN DSL DSH
干物质DM 64.54 65.67 65.88 0.312 0.171
有机物OM 65.49 65.83 66.14 0.263 0.664
粗蛋白质CP 68.34 70.58 70.09 0.489 0.138
粗脂肪EE 78.89 79.34 79.98 0.292 0.352
中性洗涤纤维NDF 56.35b 56.81b 59.33a 0.548 0.023
酸性洗涤纤维ADF 48.83 49.86 50.13 0.432 0.495

2.3 CPP对牦牛犊牛瘤胃发酵参数的影响

表4可知,DSH组总挥发性脂肪酸(TVFA)的浓度极显著高于CN组和DSL组(P<0.01),AA的浓度显著高于CN组和DSL组(P<0.05),CN组和DSL组TVFA和AA的浓度无显著差异(P≥0.05)。其余指标在各组间无显著差异(P≥0.05)。
表4 CPP对牦牛犊牛瘤胃发酵参数的影响

Table 4 Effects of CPP on rumen fermentation parameters of yak calves

项目
Items
组别Groups SEM P
P-value
CN DSL DSH
氨态氮NH3-N/(mg/dL) 10.94 10.57 11.15 0.436 0.877
乙酸AA/(mmol/L) 39.55b 46.63b 54.87a 2.511 0.011
丙酸PA/(mmol/L) 14.98 15.66 18.31 0.822 0.237
丁酸BA/(mmol/L) 6.26 6.85 7.79 0.348 0.205
异丁酸IBA/(mmol/L) 0.94 0.92 1.26 0.108 0.395
异戊酸IVA/(mmol/L) 1.51 1.47 1.69 0.078 0.551
总挥发性脂肪酸TVFA/(mmol/L) 65.67Bb 73.45Bb 85.25Aa 3.175 0.008

2.4 CPP对牦牛犊牛瘤胃微生物区系的影响

2.4.1 CPP对瘤胃微生物Alpha多样性的影响

表5可知,DSH组Shannon指数、ACE指数和Chao1指数极显著高于CN组(P<0.01),并且DSL组的ACE指数和Chao1指数极显著高于CN组(P<0.01),DSH组的ACE指数也极显著高于DSL组(P<0.01)。Shannon指数与Chao1指数在2个添加剂量组间差异不显著(P≥0.05),Simpson指数在各组间差异不显著(P≥0.05)。
表5 CPP对牦牛犊牛瘤胃微生物多样性的影响

Table 5 Effects of CPP on rumen microbiota diversity in yak calves

项目
Items
组别Groups SEM P
P-value
CN DSL DSH
Shannon指数Shannon index 5.81Bb 5.97ABab 6.23Aa 0.185 0.007
Simpson指数Simpson index 0.02 0.01 0.01 0.008 0.339
ACE指数ACE index 2 772.00Cc 3 087.00Bb 3 359.10Aa 125.100 0.001
Chao1指数Chao1 index 2 733.60Bb 3 022.20Aa 3 294.10Aa 148.810 0.002

2.4.2 CPP对瘤胃微生物Beta多样性的影响

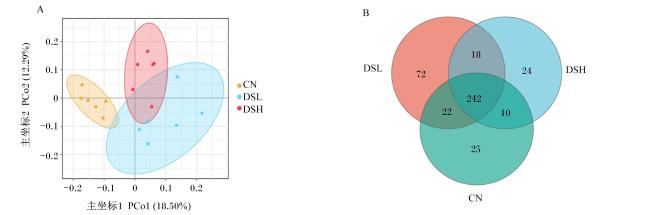
图1-A可知,主坐标1(PCo1)的差异贡献率为18.50%,主坐标2(PCo2)的差异贡献率为12.29%,CN组的样本集中分布在PCo1的负半轴和PCo2的负半轴,而DSH组的样本集中分布在PCo1的正半轴和PCo2的正半轴,各组间和组内相对分离,表明在饲粮中添加CPP对牦牛犊牛瘤胃菌群结构存在一定的影响。
图1 CPP对牦牛犊牛瘤胃微生物Beta多样性的影响及韦恩图

A:主坐标分析;B:韦恩图。CN:对照组;DSL:低剂量组;DSH:高剂量组。

Fig.1 Effects of CPP on Beta diversity of rumen microbiota in yak calves and Venn diagram

A:principal coordinates analysis;B:Venn diagram. CN:control group;DSL:low-dose group;DSH:high-dose group.

2.4.3 CPP对瘤胃微生物的分类学分析

图1-B可知,3组间共有的操作分类单元(OTU)数有242个,其中CN组特有25个OTU,DSL组特有72个OTU,DSH组特有24个OTU。这说明在饲粮中添加CPP改变了牦牛犊牛的瘤胃微生物结构。

2.4.4 CPP对瘤胃微生物物种分类学的影响

表6可知,在门水平上,厚壁菌门和拟杆菌门是犊牛瘤胃菌群中的优势菌门,DSH组髌骨细菌门的相对丰度与CN组和DSL组相比有升高的趋势(P=0.050)。
表6 CPP对牦牛犊牛瘤胃微生物相对丰度的影响

Table 6 Effects of CPP on relative abundance of rumen microbiota in yak calves %

项目
Items
组别Groups SEM P
P-value
CN DSL DSH
门Phylum
厚壁菌门Firmicutes 58.19 60.01 55.89 1.620 0.610
拟杆菌门Bacteroidetes 37.16 35.04 38.02 1.573 0.752
放线菌门Actinobacteria 1.50 1.80 1.72 0.208 0.850
髌骨细菌门Patescibacteria 1.36 1.12 1.82 0.122 0.050
螺旋体门Spirochaetes 0.94 1.00 1.37 0.122 0.314
疣微菌门Verrucomicrobia 0.17 0.26 0.32 0.031 0.165
热脱硫杆菌门Thermodesulfobacteria 0.18 0.17 0.19 0.021 0.949
未分类细菌
Unclassified_k_norank_d_Bacteria
0.16 0.17 0.20 0.019 0.710
变形菌门Proteobacteria 0.14 0.15 0.16 0.010 0.734
纤维杆菌门Fibrobacteres 0.07 0.11 0.15 0.017 0.212
绿弯菌门Chloroflexi 0.08 0.11 0.11 0.014 0.647
蓝细菌门Cyanobacteria 0.01 0.03 0.02 0.010 0.545
其他Others 0.04 0.04 0.05 0.005 0.526
属Genus
理研菌科RC9肠道群
Rikenellaceae_RC9_gut_group
12.50 12.31 13.50 0.526 0.639
未明确科的F082 Norank_f_F082 9.76 7.89 11.13 0.653 0.123
克里斯滕森菌科R-7群
Christensenellaceae_R-7_group
8.36 7.95 7.18 0.442 0.573
NK4A214群NK4A214_group 6.55 6.42 6.68 0.408 0.970
草酸杆菌属Oxalobacter 7.99 5.62 5.23 1.134 0.591
未明确科的UCG-011
Norank_f_UCG-011
5.45 4.98 4.13 0.522 0.605
毛螺菌科-NK3A20群
Lachnospiraceae_NK3A20_group
2.65 2.58 2.85 0.274 0.923
UCG-005 1.71 4.30 2.05 0.832 0.409
未分类梭菌纲UCG-014
Norank_o_Clostridia_UCG-014
2.37 2.21 2.27 0.196 0.952
产乙酸糖发酵菌属Saccharofermentans 1.94 1.87 2.40 0.174 0.431
瘤胃球菌属Ruminococcus 1.17Bb 1.39ABab 3.20Aa 0.310 0.005
未明确科的UCG-010
Norank_f_UCG-010
1.63 2.42 1.59 0.248 0.326
未分类瘤胃球菌科
Unclassified_f_Ruminococcaceae
4.26 0.42 0.73 1.231 0.390
未明确科的穆里氏菌科
Norank_f_Muribaculaceae
1.38 1.19 1.73 0.159 0.397
候选糖单胞菌属Candidatus_Saccharimonas 1.05b 1.33ab 1.78a 0.116 0.026
其他Others 30.73 37.63 33.54 1.349 0.105
表6可知,在属水平上,理研菌科RC9肠道群、未明确科的F082和其他菌属是犊牛瘤胃菌群中的优势菌属。此外,DSH组瘤胃球菌属的相对丰度极显著高于CN组(P<0.01),候选糖单胞菌属的相对丰度显著高于CN组(P<0.05)。其余菌属的相对丰度在各组间差异均不显著(P≥0.05)。

2.4.5 CPP对牦牛犊牛瘤胃菌群代谢途径和功能预测分析

表7可知,在KEGG生物代谢二级通路水平上,牦牛犊牛的脂质代谢通路及折叠、分类和降解通路在DSH组极显著富集(P<0.01),辅酶和维生素代谢、萜类和聚酮类代谢及其他氨基酸代谢通路在DSH组显著富集(P<0.05)。而对COG通路进行富集分析后发现,各通路在各组间无显著差异(P≥0.05)。
表7 KEGG功能通路和COG功能通路

Table 7 KEGG functional pathway and COG functional pathway

项目
Items
组别Groups SEM P
P-value
CN DSL DSH
KEGG通路富集分析KEGG pathway enrichment analysis
脂质代谢Lipid metabolism 0.57Bb 0.61Aa 0.64Aa 0.010 0.006
辅酶和维生素代谢
Metabolism of coenzymes and vitamins
0.36ab 0.33b 0.38a 0.007 0.020
萜类和聚酮类代谢
Metabolism of terpenoids and polyketides
0.53b 0.54b 0.59a 0.009 0.013
其他氨基酸的代谢
Metabolism of other amino acids
0.32b 0.31b 0.36a 0.008 0.016
折叠、分类和降解
Folding, sorting and degradation
0.61Bb 0.62Bb 0.68Aa 0.011 0.008
COG通路富集分析COG pathway enrichment analysis
细胞壁/膜/包膜生物合成
Cell wall/membrane/envelope biogenesis
7.34 7.13 7.38 0.298 0.544
复制,重组和修复
Replication, recombination and repair
6.20 6.17 6.20 0.103 0.754
细胞内运输、分泌和囊泡运输
Intracellular trafficking, secretion,
and vesicular transport
1.32 1.33 1.34 0.027 0.290

2.4.6 饲粮相关性状和瘤胃挥发性脂肪酸与瘤胃微生物及代谢通路的相关性分析
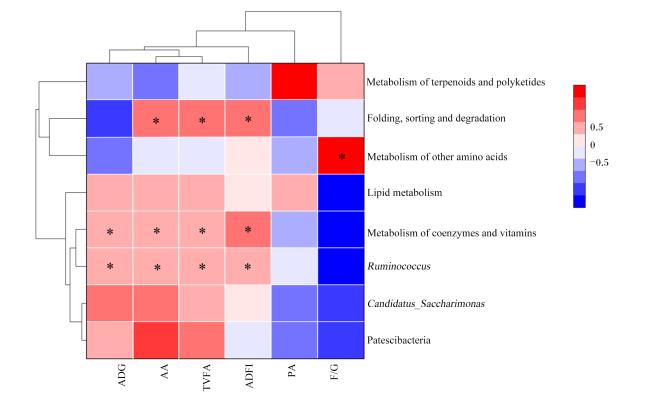
图2可知,ADG、ADFI和TVFA、AA的浓度与瘤胃球菌属相对丰度、辅酶和维生素代谢通路呈显著正相关(P<0.05),此外,ADFI和TVFA、AA的浓度与折叠、分类和降解通路呈显著正相关(P<0.05)。F/G与其他氨基酸的代谢通路呈显著正相关(P<0.05)。
图2 饲粮相关性状、瘤胃挥发性脂肪酸与瘤胃微生物及代谢通路相关性分析

ADG:平均日增重 average daily gain;AA:乙酸 acetic acid;TVFA:总挥发性脂肪酸total volatile fatty acid;ADFI:平均日采食量 average daily feed intake;PA:丙酸 propionic acid;F/G:料重比 feed to gain ratio;Metabolism of terpenoids and polyketides:萜类和聚酮类代谢;Folding, sorting and degradation:折叠、分类和降解;Metabolism of other amino acids:其他氨基酸的代谢;Lipid metabolism:脂质代谢;Metabolism of coenzymes and vitamins:辅酶和维生素代谢;Ruminococcus:瘤胃球菌属;Patescibacteria:髌骨细菌门;Candidatus_Saccharimonas:候选糖单胞菌属。

*为显著相关(P<0.05)。* is significantly correlated (P<0.05).

Fig.2 Correlation analysis of feed-related traits, rumen VFA with rumen microbiota and metabolic pathways

3 讨论

3.1 CPP对牦牛犊牛生长性能和养分消化率的影响

动物的生长发育过程主要是机体对营养物质消化、吸收和利用,最后在体内沉积的结果[17]。补饲可以为反刍动物提供额外生长所必需的营养物质,并提升饲料利用率和养殖效益。犊牛的总增重和ADG直接反映其生长速度与健康状况,影响未来生长性能。本试验中,DSH组FBW、ADG和ADFI显著高于CN组,F/G也有下降的趋势。这说明牦牛犊牛饲粮中添加CPP能够提高犊牛的生长性能,原因可能是CPP能够改善犊牛的瘤胃肠道健康与消化能力,提高营养物质利用率,进而提高ADG。本试验中,CPP可以提高NDF消化率的结果证明了这一点。这与尹莉莉[18]在仔猪,贺丽茹等[19]和石轶男等[20]在肉仔鸡以及李开菊等[21]在乌鸡的研究中CPP可显著提高动物ADG、ADFI和降低F/G的结果一致。
养分消化率是衡量饲料消化性和动物消化能力的第1指标,它受动物品种、年龄、饲粮及环境等的影响。本试验中,高剂量CPP可显著提高犊牛NDF消化率,说明CPP的添加可改善犊牛的纤维消化能力。有研究表明,瘤胃球菌属作为重要的纤维素降解菌属,具有分泌较高稳定性和耐热性纤维素酶的作用,从而能高效降解抗性淀粉和纤维素[22-23],且犊牛瘤胃内瘤胃球菌属相对丰度的升高更加剧了纤维素的降解效率,进而使NDF消化率显著提高。CPP由重要的单糖和单糖衍生物组成,如甘露聚糖、阿拉伯糖、鼠李糖、葡萄糖和半乳糖等[24]。王昭喆等[25]在肉牛、梁煜翔等[26]在猪的研究表明,发酵棕榈粕(主要成分是甘露聚糖)可显著提高NDF消化率。结合本试验中生长性能和养分消化的结果,可以说明CPP可能是因为提高了NDF的消化率,从而使牦牛沉积的养分更多,生长发育更好。

3.2 CPP对牦牛犊牛瘤胃发酵参数的影响

挥发性脂肪酸作为反刍动物瘤胃发酵中的重要产物,是反刍动物重要的能量来源。在TVFA中AA的浓度最高,占其总产量的70%~75%[27],它是合成乳脂和体脂的主要前体物质,还可氧化释放能量[28],并且体现了瘤胃发酵特征和营养物质降解效率[29]。本试验中,DSH组TVFA的浓度极显著高于CN组和DSL组,AA的浓度也显著高于CN组和DSL组,说明添加高剂量的CPP有利于促进瘤胃发酵,产生更多的VFA,并且更有利于AA发酵。其原因可能是CPP的饲喂使犊牛瘤胃菌群发生了变化,导致如瘤胃球菌等纤维素分解菌的相对丰度升高,使瘤胃降解纤维素的能力增强,进而增加了AA的浓度[30]。这与王广[31]和Fu等[32]的研究结果中CPP能显著提高小鼠结肠和盲肠内的AA浓度相似。

3.3 CPP对牦牛犊牛瘤胃微生物区系的影响

瘤胃微生物对饲粮中营养物质消化和反刍动物机体功能的维持有重要作用[33]。反刍动物为瘤胃微生物提供了适宜的生长环境,而微生物则在瘤胃中分解营养物质,以供反刍动物吸收和利用[34],主要包括原虫、细菌和真菌,它们在瘤胃内形成了稳定的生态环境[35]。一般来说,微生物多样性和丰富度越高,微生物群落结构就越稳定[36]。Alpha多样性指数分析中,Shannon指数和Simpson指数与微生物多样性相关,ACE指数和Chao1指数常用于估计物种的丰富度。在本试验中,DSH组Shannon指数、ACE指数和Chao1指数极显著高于CN组,这说明CPP能提高瘤胃微生物多样性并增加丰富度。这与陈新君[37]和Yang等[38]在小鼠中的研究结果一致,即CPP可显著提高小鼠结肠内Shannon指数和Chao1指数。
通过对门水平的分类鉴别和比较,笔者统计了排列水平在前12位的差异物种,发现犊牛瘤胃中厚壁菌门和拟杆菌门占瘤胃微生物总相对丰度的90%以上,为犊牛瘤胃微生物中的优势菌门。而各组间优势菌门并无显著差异,表明CPP的添加并未影响犊牛瘤胃微生物区系的组成。这与Zhang等[39]在绵羊中的研究结果一致。在本试验中,DSH组髌骨细菌门的相对丰度较CN、DSL组有上升趋势。髌骨细菌主要存在于生物膜中,在高海拔环境下可能通过非厌氧呼吸发酵丙酮酸产生AA、乳酸和甲酸等,为肠道细胞的自我保护提供能量并维持能量平衡[40-41]。此外,它分泌的碳水化合物活性酶还能帮助分解难以消化的植物成分,间接促进纤维发酵[42]。在属水平上发现,排列位次于前15的差异物种中,其他菌属、理研菌科RC9肠道群和未明确科的F082为优势菌属。本试验中,DSH组犊牛的瘤胃球菌属和候选糖单胞菌属的相对丰度显著高于CN组。瘤胃球菌属是一种潜在的益生菌,具有促进消化等多种积极作用,能够将纤维素分解为可被瘤胃中其他菌群利用的简单糖类,并产生挥发性脂肪酸[43],本试验中,CPP促进了犊牛对纤维素的分解回应了以上结果。有研究发现,候选糖单胞菌属是一种可以产生短链脂肪酸的有益菌,进而起到增加肠道通透性,保持瘤胃微生物系统稳定的作用,为瘤胃微生物的正常生长代谢创造良好的环境[44],还能提高反刍动物对营养物质的吸收效率[45]。以上结果表明,饲粮中添加高剂量的CPP可提高犊牛瘤胃对纤维素的分解能力,提高生长性能,同时有助于维持瘤胃的正常功能和微生物区系的稳定。
通过KEGG通路分析,发现3组牦牛犊牛代谢产物的差异富集主要集中在脂质代谢与辅酶和维生素代谢等途径。脂质是反刍动物能量供应和细胞膜合成的重要物质。DSH组脂质代谢通路的富集可能与瘤胃球菌属等纤维素降解菌的丰度增加有关,这些菌群通过分解纤维产生挥发性脂肪酸,进而为脂质合成提供前体物质[46]。辅酶和维生素是动物体内多种代谢过程的重要辅助因子,其代谢通路的富集可能有助于提高能量转化效率和抗氧化作用[47],使犊牛能够更有效地利用营养物质,并且减少外界因素对机体的损伤。这些结果表明,CPP可能通过调节瘤胃微生物代谢活性,增强了瘤胃微生物的功能,从而促进营养物质的分解与利用。
通过对饲粮相关性状与瘤胃微生物的相关性分析发现,犊牛的ADG和ADFI与瘤胃球菌属相对丰度呈显著正相关。瘤胃球菌属作为瘤胃内肠道微生物的重要组成部分,能有效地分解碳水化合物,产生AA、甲酸和少量乳酸等代谢产物[48]。因此,随着瘤胃球菌数量的增加,其营养代谢活动更为活跃,使得AA的生成量也随之增加。折叠、分类和降解通路涉及到蛋白质等生物大分子的处理过程[49]。在本试验中,TVFA和AA的浓度与折叠、分类和降解通路呈显著正相关,这可能说明当瘤胃内AA浓度较高时,瘤胃微生物的生长代谢活动增强,加快了蛋白质的降解速率[50]。然而,关于这些菌种对瘤胃发酵和生长性能具体的影响机制仍需进一步研究。

4 结论

饲粮中添加CPP在一定程度上增加了牦牛犊牛的瘤胃微生物多样性和丰富度,改变了瘤胃微生物结构,提高了厚壁菌门及瘤胃球菌属等微生物的相对丰度,并富集脂质代谢、辅酶和维生素代谢、萜类和聚酮类代谢、其他氨基酸代谢以及折叠、分类和降解通路,促进了瘤胃发酵,提高了瘤胃TVFA的浓度和纤维消化,从而提高了犊牛的生长性能。
[1]
孟庆辉, 陈永杏, 董红敏, 等. 牦牛分布特点及其种群数量[J]. 家畜生态学报, 2017, 38(3):80-85.

MENG Q H, CHEN Y X, DONG H M, et al. The distribution characteristics and populations of yak[J]. Acta Ecologae Animalis Domastici, 2017, 38(3):80-85. (in Chinese)

[2]
HALFEN J, CARPINELLI N, DEL PINO F A B, et al. Effects of yeast culture supplementation on lactation performance and rumen fermentation profile and microbial abundance in mid-lactation Holstein dairy cows[J]. Journal of Dairy Science, 2021, 104(11):11580-11592.

DOI

[3]
李芳, 杨扶德. 党参多糖提取分离、化学组成和药理作用研究进展[J]. 中华中医药学刊, 2023, 41(4):42-49.

LI F, YANG F D. Research progress on extraction and isolation,chemical compound and pharmacological effects of polysaccharide from Dangshen (Codonopsis radix)[J]. Chinese Archives of Traditional Chinese Medicine, 2023, 41(4):42-49. (in Chinese)

[4]
毋玲玲, 魏玉杰, 张兆萍, 等. 甘肃省中药材生态种植模式调查整理及问题与对策分析[J]. 中药材, 2025, 48(2):269-273.

WU L L, WEI Y J, ZHANG Z P, et al. Investigation and arrangement of ecological planting patterns of Chinese medicinal materials in Gansu province and analysis of problems and countermeasures[J]. Journal of Chinese Medicinal Materials, 2025, 48(2):269-273. (in Chinese)

[5]
时军, 马方励, 王晓燕, 等. 党参药材中党参炔苷与总多糖、总皂苷含量的相关性研究[J]. 中华中医药学刊, 2011, 29(12):2779-2781.

SHI J, MA F L, WANG X Y, et al. Correlation of lobetyolin,total polysaccharides and total saponins from different region of Radix Codonopsis[J]. Chinese Archives of Traditional Chinese Medicine, 2011, 29(12):2779-2781. (in Chinese)

[6]
YANG C X, GOU Y Q, CHEN J Y, et al. Structural characterization and antitumor activity of a pectic polysaccharide from Codonopsis pilosula[J]. Carbohydrate Polymers, 2013, 98(1):886-895.

DOI

[7]
李启艳, 祝清芬, 刘春霖, 等. 党参多糖分离纯化及抗氧化活性研究[J]. 中草药, 2017, 48(5):907-912.

LI Q Y, ZHU Q F, LIU C L, et al. Isolation and purification of Codonopsis pilosula polysaccharide and its anti-oxidant activity[J]. Chinese Traditional and Herbal Drugs, 2017, 48(5):907-912. (in Chinese)

[8]
胡家耀. 党参多糖对奶牛生产性能、抗氧化指标和免疫功能的影响[J]. 中国奶牛, 2025,(5):24-28.

HU J Y. The effects of Codonopsis pilosula polysaccharides on the production performance,antioxidant indicators,and immune function of cows[J]. China Dairy Cattle, 2025,(5):24-28. (in Chinese)

[9]
隋奉桐, 陈静, 马旭东, 等. 党参多糖对断奶仔猪生长性能、血清免疫指标及抗氧化指标的影响[J]. 饲料工业, 2024, 45(7):38-42.

SUI F T, CHEN J, MA X D, et al. Effects of Codonopsis polysaccharides on growth performance,serum immunity indexes and antioxidant indexes of weaned piglets[J]. Feed Industry, 2024, 45(7):38-42. (in Chinese)

[10]
TANG S, LIU W, ZHAO Q Q, et al. Combination of polysaccharides from Astragalus membranaceus and Codonopsis pilosula ameliorated mice colitis and underlying mechanisms[J]. Journal of Ethnopharmacology, 2021, 264:113280.

[11]
孙嘉琪. 硫酸化党参多糖对巨噬细胞及小鼠急性氧化损伤的保护作用[D]. 硕士学位论文. 广州: 华南农业大学, 2018.

SUN J Q. Protective effect of sulfated Codonopsis pilosula polysaccharide on oxidative injury in macrophages and mice[D]. Master’s Thesis. Guangzhou: South China Agricultural University, 2018. (in Chinese)

[12]
ZHANG P, HU L H, BAI R B, et al. Structural characterization of a pectic polysaccharide from Codonopsis pilosula and its immunomodulatory activities in vivo and in vitro[J]. International Journal of Biological Macromolecules, 2017, 104(Pt A):1359-1369.

DOI

[13]
ZHOU J X, YANG Q X, WEI W F, et al. Codonopsis pilosula polysaccharide alleviates ulcerative colitis by modulating gut microbiota and SCFA/GPR/NLRP3 pathway[J]. Journal of Ethnopharmacology, 2025, 337(Pt 2):118928.

DOI

[14]
MATHEW B, EASTRIDGE M L, OELKER E R, et al. Interactions of monensin with dietary fat and carbohydrate components on ruminal fermentation and production responses by dairy cows[J]. Journal of Dairy Science, 2011, 94(1):396-409.

DOI PMID

[15]
冯宗慈, 高民. 通过比色测定瘤胃液氨氮含量方法的改进[J]. 畜牧与饲料科学, 2010, 31(6/7):37.

FENG Z C, GAO M. Improvement of the method for determining the ammonia-nitrogen content of rumen liquor by colourimetry[J]. Animal Husbandry and Feed Science, 2010, 31(6/7):37. (in Chinese)

[16]
LI Z P, WRIGHT A D G, LIU H L, et al. Response of the rumen microbiota of sika deer (Cervus nippon) fed different concentrations of tannin rich plants[J]. PLoS One, 2015, 10(5):e0123481.

DOI

[17]
张振宇, 梁春年, 姚喜喜, 等. 日粮不同营养水平对牦牛生产性能、屠宰指标和血清生化指标的影响[J]. 畜牧兽医学报, 2021, 52(1):135-143.

DOI

ZHANG Z Y, LIANG C N, YAO X X, et al. Effects of different nutrition levels of diets on production performance,slaughter indexes and serum biochemical indexes of yak[J]. Acta Veterinaria et Zootechnica Sinica, 2021, 52(1):135-143. (in Chinese)

[18]
尹莉莉. 党参多糖对仔猪免疫机能的影响[D]. 硕士学位论文. 合肥: 安徽农业大学, 2016.

YIN L L. Effects of Codonopsis pilosula polysaccharide on immune function in piglets[D]. Master’s Thesis. Hefei: Anhui Agricultural University, 2016. (in Chinese)

[19]
贺丽茹, 张梅. 党参多糖对肉鸡生产性能、肉品质及肌肉氨基酸组成的影响[J]. 中国饲料, 2025,(6):1-4.

HE L R, ZHANG M. The effect of Codonopsis polysaccharides on the production performance,meat quality,and muscle amino acid composition of broiler chickens[J]. China Feed, 2025,(6):1-4. (in Chinese)

[20]
石轶男, 杨绒娟, 妍妍, 等. 党参多糖可溶性粉对肉仔鸡血清ND抗体水平、IgG及肠道SIgA含量的影响[J]. 中国兽药杂志, 2016, 50(9):47-52.

SHI Y N, YANG R J, YAN Y, et al. Effects of Codonopsis pilosula polysaccharides soluble powder on broiler serum antibody level of ND,IgG and intestinal SIgA content[J]. Chinese Journal of Veterinary Drug, 2016, 50(9):47-52. (in Chinese)

[21]
李开菊, 陈文倩, 周霞, 等. 素花党参多糖对乌鸡生长性能、免疫功能、血常规及肠道菌群的影响[J]. 四川畜牧兽医, 2017, 44(10):32-34,36.

LI K J, CHEN W Q, ZHOU X, et al. Effects of Codonopsis pilosula polysaccharides on the production performance,immune function,routine blood indexes and intestinal microflora of black-bone chicken[J]. Sichuan Animal & Veterinary Sciences, 2017, 44(10):32-34,36. (in Chinese)

[22]
李敏. 瘤胃纤维素降解细菌和真菌的互作对纤维物质降解的影响[D]. 硕士学位论文. 呼和浩特: 内蒙古农业大学, 2015.

LI M. Interaction of the ruminal cellulose-degrading bacteria and fungi with fiber degradation[D]. Master’s Thesis. Hohhot: Inner Mongolia Agricultural University, 2015. (in Chinese)

[23]
HODA A, TAFAJ M, SALLAKU E. In silico structural,functional and phylogenetic analyses of cellulase from Ruminococcus albus[J]. Journal of Genetic Engineering and Biotechnology, 2021, 19(1):58.

DOI

[24]
黄延盛, 张欣, 刘耀军, 等. 我国不同产地党参药材中糖类成分比较分析[J]. 南昌大学学报(工科版), 2022, 44(4):326-334.

HUANG Y S, ZHANG X, LIU Y J, et al. Comparison on sugar composition in Codonopsis pilosula from different regions in China[J]. Journal of Nanchang University(Engineering & Technology), 2022, 44(4):326-334. (in Chinese)

[25]
王昭喆, 肖海翔, 姜奥宇, 等. 发酵棕榈粕替代部分玉米和豆粕对肉牛生长性能、养分表观消化率、血清生化指标及瘤胃发酵参数的影响[J]. 动物营养学报, 2025, 37(3):1858-1867.

DOI

WANG Z Z, XIAO H X, JIANG A Y, et al. Effects of partially replacing corn and soybean meal with fermented palm kernel meal on growth performance,nutrient apparent digestibility,serum biochemical indices and rumen fermentation parameters of beef cattle[J]. Chinese Journal of Animal Nutrition, 2025, 37(3):1858-1867. (in Chinese)

[26]
梁煜翔, 孙耀威, 李凯, 等. 棕榈粕饲粮对生长猪生长性能、养分表观消化率和抗氧化功能的影响[J]. 动物营养学报, 2025, 37(3):1632-1644.

DOI

LIANG Y X, SUN Y W, LI K, et al. Effects of palm kernel cake diet on growth performance,nutrient apparent digestibility and antioxidant function in growing pigs[J]. Chinese Journal of Animal Nutrition, 2025, 37(3):1632-1644. (in Chinese)

[27]
杨春涛, 刁其玉, 司丙文, 等. 挥发性脂肪酸在反刍动物瘤胃上皮吸收转运及调节作用[J]. 中国畜牧杂志, 2015, 51(7):78-83.

YANG C T, DIAO Q Y, SI B W, et al. Absorption and regulation of volatile fatty acids in the ruminal epithelium[J]. Chinese Journal of Animal Science, 2015, 51(7):78-83. (in Chinese)

[28]
LI M, ZHANG X J, AGRAWAL A, et al. Effect of acetate formation pathway and long chain fatty acid CoA-ligase on the free fatty acid production in E.coli expressing acy-ACP thioesterase from Ricinus communis[J]. Metabolic Engineering, 2012, 14(4):380-387.

DOI

[29]
ESLAM A, BELGUTEI B, NAOKI F, et al. Evaluation of different brown seaweeds as feed and feed additives regarding rumen fermentation and methane mitigation[J]. Fermentation, 2022, 8(10):504.

DOI

[30]
王海玉, 赵苗苗, 左艳华, 等. 复合益生菌对羔羊营养物质表观消化率、瘤胃发酵参数和微生物区系的影响[J]. 动物营养学报, 2025, 37(5):3180-3193.

DOI

WANG H Y, ZHAO M M, ZUO Y H, et al. Effects of complex probiotics on nutrient apparent digestibility,rumen fermentation parameters and microbiota of lambs[J]. Chinese Journal of Animal Nutrition, 2025, 37(5):3180-3193. (in Chinese)

[31]
王广. 党参多糖对肠道菌群失调小鼠的调整作用机制的初步研究[D]. 硕士学位论文. 佳木斯: 佳木斯大学, 2010.

WANG G. Preliminary study on the mechanism of adjusting effect of Codonopsis pilosula polysaccharides on mice with dysbiosis of intestinal flora[D]. Master’s Thesis. Jiamusi: Jiamusi University, 2010. (in Chinese)

[32]
FU Y P, FENG B, ZHU Z K, et al. The polysaccharides from Codonopsis pilosula modulates the immunity and intestinal microbiota of cyclophosphamide-treated immunosuppressed mice[J]. Molecules, 2018, 23(7):1801.

DOI

[33]
袁金泉, 别欣亚, 周亚楠, 等. 精粗分饲与颗粒型混合饲粮对断奶牦牛犊牛生长性能、养分表观消化率和瘤胃功能的影响[J]. 动物营养学报, 2025, 37(7):4634-4650.

DOI

YUAN J Q, BIE X Y, ZHOU Y N, et al. Effects of separate concentrate and forage and pelleted mixed diet on growth performance,nutrient apparent digestibility and rumen function of weaned yak calves.[J]. Chinese Journal of Animal Nutrition, 2025, 37(7):4634-4650. (in Chinese)

[34]
MALMUTHUGE N, GUAN L L. Understanding host-microbial interactions in rumen:searching the best opportunity for microbiota manipulation[J]. Journal of Animal Science and Biotechnology, 2017, 8:8.

[35]
MAO H L, ZHANG Y F, YUN Y, et al. Weaning age affects the development of the ruminal bacterial and archaeal community in Hu lambs during early life[J]. Frontiers in Microbiology, 2021, 12:636865.

[36]
PETERSEN C, ROUND J L. Defining dysbiosis and its influence on host immunity and disease[J]. Cellular Microbiology, 2014, 16(7):1024-1033.

DOI PMID

[37]
陈新君. 复方四君子汤及党参多糖调节溃疡性结肠炎小鼠肠道菌群的作用研究[D]. 硕士学位论文. 兰州: 兰州大学, 2016.

CHEN X J. Sijunzi decoction and Codonopsis pilosula polysaccharide alleviate DSS-induced mice colitis by modulating gut microbiota[D]. Master’s Thesis. Lanzhou: Lanzhou University, 2016. (in Chinese)

[38]
YANG M J, LV J H, YANG J M, et al. Effects of Codonopsis pilosula crude polysaccharides by hypoglycemic and modulating gut microbiome in a high-fat diet and streptozotocin-induced mouse model of T2DM[J]. Journal of Functional Foods, 2023, 111:105893.

[39]
ZHANG Y K, ZHANG X X, LI F D, et al. Characterization of the rumen microbiota and its relationship with residual feed intake in sheep[J]. Animal, 2021, 15(3):100161.

DOI

[40]
陶晔, 邢鹏. 候选门级辐射类群(CPR)细菌研究进展[J]. 微生物学报, 2020, 60(6):1284-1303.

TAO Y, XING P. Progress in candidate phyla radiation (CPR) research[J]. Acta Microbiologica Sinica, 2020, 60(6):1284-1303. (in Chinese)

[41]
WANG X B, WU X Y, SHANG Y Q, et al. High-altitude drives the convergent evolution of alpha diversity and indicator microbiota in the gut microbiomes of ungulates[J]. Frontiers in Microbiology, 2022, 13:953234.

[42]
CHANG Z Y, LIU H M, LEU Y L, et al. Modulation of gut microbiota combined with upregulation of intestinal tight junction explains anti-inflammatory effect of corylin on colitis-associated cancer in mice[J]. International Journal of Molecular Sciences, 2022, 23(5):2667.

DOI

[43]
朱振宇, 杨成, 王明根, 等. 屎肠球菌F11.1G菌剂对断奶羔羊生长性能、营养物质表观消化率、屠宰性能、瘤胃发酵和瘤胃微生物区系的影响[J]. 动物营养学报, 2024, 36(5):3143-3155.

DOI

ZHU Z Y, YANG C, WANG M G, et al. Effects of Enterococcus faecium F11.1G on growth performance,nutrient apparent digestibility,slaughter performance,rumen fermentation and rumen microflora of weaned lambs[J]. Chinese Journal of Animal Nutrition, 2024, 36(5):3143-3155. (in Chinese)

[44]
ZENG Z, TONG X L, YANG Y, et al. Pediococcus pentosaceus ZZ61 enhances growth performance and pathogenic resistance of silkworm Bombyx mori by regulating gut microbiota and metabolites[J]. Bioresource Technology, 2024, 402:130821.

[45]
OGUNADE I, SCHWEICKART H, MCCOUN M, et al. Integrating 16S rRNA sequencing and LC-MS-based metabolomics to evaluate the effects of live yeast on rumen function in beef cattle[J]. Animals, 2019, 9(1):28.

DOI

[46]
CONTE G, DIMAURO C, DAGHIO M, et al. Exploring the relationship between bacterial genera and lipid metabolism in bovine rumen[J]. Animal, 2022, 16(5):100520.

DOI

[47]
辜雪冬. 基于多组学的藏猪与约克夏猪肝脏对不同海拔的响应通路研究[D]. 博士学位论文. 拉萨: 西藏大学, 2024.

GU X D. Study on response pathway of Tibetan pig yorkshire pig liver to different altitudes based on multiomics[D]. Ph.D.Thesis. Lhasa: Tibet University, 2024. (in Chinese)

[48]
贾子悦, 钟丽媛, 薛茗元, 等. 饲喂含秸秆发酵饲料对育成牛瘤胃微生物组成和功能的影响[J]. 浙江大学学报(农业与生命科学版), 2024, 50(4):517-530.

JIA Z Y, ZHONG L Y, XUE M Y, et al. Effect of feeding straw-containing fermented feed on the composition and function of the rumen microbiota in heifers[J]. Journal of Zhejiang University (Agriculture & Life Sciences), 2024, 50(4):517-530. (in Chinese)

[49]
HEBERT D N, MOLINARI M. In and out of the ER:protein folding, quality control,degradation,and related human diseases[J]. Physiological Reviews, 2007, 87(4):1377-1408.

DOI

[50]
CAO N, WU H, ZHANG X Z, et al. Calcium propionate supplementation alters the ruminal bacterial and archaeal communities in pre- and postweaning calves[J]. Journal of Dairy Science, 2020, 103(4):3204-3218.

DOI PMID

Outlines

/