REVIEW

Research Progress on Lactobacillus reuteri in Piglet Production: Growth Performance and Intestinal Health

  • ZHANG Yiting , 1, 2 ,
  • CUI Chenbin , 1, * ,
  • SUN Jinhua 2 ,
  • YANG Xuefen 1
Expand
  • 1 Guangdong Provincial Key Laboratory of Animal Breeding and Nutrition, Key Laboratory of Animal Nutrition and Feed Science in South China, Ministry of Agriculture and Rural Affairs, State Key Laboratory of Swine and Poultry Breeding Industry, Institute of Animal Science, Guangdong Academy of Agricultural Sciences, Guangzhou 510640, China
  • 2 College of Animal Science and Technology, Northeast Agricultural University, Harbin 150030, China
*assistant professor, E-mail:

Received date: 2025-08-14

  Online published: 2026-03-16

Abstract

Lactobacillus reuteri is widely colonized in the mammal intestines, breast milk and natural environment. As one of the most extensively studied probiotics, it exerts broad application prospects in the field of animal health due to its unique biological characteristics. Recent studies have confirmed its diverse functional characteristics in piglet production, including growth performance elevation and intestinal health improvement. However, there is currently a lack of systematic comparison of the effects of different strains, dosages, and addition methods of Lactobacillus reuteri. The research on its action targets and mechanisms, as well as the safety research on long-term use, remains insufficiently in-depth. This paper systematically reviewed the latest research progress on Lactobacillus reuteri in enhancing piglet growth performance, regulating intestinal health, and modulating immunity, aiming to provide valuable references for developing new probiotic formulations and innovative ideas for achieving green farming.

Cite this article

ZHANG Yiting , CUI Chenbin , SUN Jinhua , YANG Xuefen . Research Progress on Lactobacillus reuteri in Piglet Production: Growth Performance and Intestinal Health[J]. Chinese Journal of Animal Nutrition, 2026 , 38(3) : 1612 -1623 . DOI: 10.12418/CJAN2026.129

在全球畜牧业中,抗生素的广泛使用引发了细菌耐药性增强、药物残留超标及动物肠道菌群失调等问题,严重威胁动物健康与食品安全。为应对这一挑战,多个国家已实施“禁抗”政策。在此背景下,寻找安全、有效的抗生素替代品成为畜牧业面临的关键课题。益生菌凭借其天然性和无有害残留物的特性,被广泛认为是具有潜力的抗生素替代物。目前,被发现的益生菌种类繁多,包括乳杆菌属、双歧杆菌属、丙酸杆菌属、链球菌属、芽孢杆菌属和肠球菌属等[1]。其中,乳杆菌属作为使用最广泛的益生菌之一,在各类食品和动物饲料添加剂中占据重要地位[2]
乳杆菌属广泛存在于自然界中,目前从人、小鼠和猪等物种粪便中分离出了多种乳杆菌。在仔猪生产领域,罗伊氏乳杆菌(Lactobacillus reuteri)的应用价值尤为突出,其已被证明可有效提高仔猪的生长性能,包括提高日增重、降低死亡率以及减少腹泻等效果[3-4];并且能通过调节免疫反应、增强肠道屏障完整性、平衡肠道微生物群落和缓解炎症反应,从而显著改善仔猪肠道健康,为仔猪健康生长提供多维度保障[5-7]。因此,本文旨在系统综述罗伊氏乳杆菌对仔猪生长性能和肠道健康的研究进展,以期为该菌在畜禽生产中的深入研究和应用提供参考与思路。

1 罗伊氏乳杆菌概述

乳杆菌属为革兰氏阳性菌,因可通过发酵代谢途径生成乳酸而得名[8]。常见的乳杆菌包括罗伊氏乳杆菌、约氏乳杆菌、植物乳杆菌、嗜酸乳杆菌、加氏乳杆菌、鼠李糖乳杆菌、保加利亚乳杆菌和发酵乳杆菌等。其中,罗伊氏乳杆菌因其独特的生理功能和广泛的宿主适应性,受到了广泛关注[9]。罗伊氏乳杆菌属于乳杆菌属,是革兰氏阳性且厌氧或兼性厌氧的杆状细菌。该菌呈微弯杆状,末端钝圆,适宜生长温度为35~40 ℃,适宜pH为6.7~7.0[10]。此外,罗伊氏乳杆菌对酸和胆盐具有较高的耐受性[11],并表现出较强的疏水性和聚集特性[12],这些特性使其能够适应并顺利定植于胃肠道的严苛环境[13]。罗伊氏乳杆菌具有显著的宿主特异性,目前已从各种动物的胃肠道中分离出多种菌株,且针对不同物种来源的罗伊氏乳杆菌均有大量的研究[14-17]。作为动物肠道中最常见的乳杆菌之一,罗伊氏乳杆菌可通过靶向定植、分泌代谢产物[18]及调控信号通路等机制[19],发挥促进生长[20]、调节免疫[5]、改善肠道屏障功能[21]和重塑肠道菌群稳态[6]等多重益生作用,有效促进仔猪生长发育。
罗伊氏乳杆菌的安全性已获得欧洲食品安全局的权威认证,被列入“安全资格推定”推荐清单[22]。临床研究证实,罗伊氏乳杆菌菌株ATCC PTA 4659和DSM 17938在健康人群中安全性和耐受性良好[23-24],健康成年人每日摄入5×10⁸ CFU的罗伊氏乳杆菌DSM 17938,持续2个月,安全且耐受性良好,无严重不良事件[23];罗伊氏乳杆菌ATCC PTA 4659的系统性安全评估表明,其基因组不含毒力及耐药基因,且健康成年人即使每日摄入高达1×10¹¹ CFU的剂量也被证明是安全的[24]。这些研究共同表明,经过严格筛选和评估的罗伊氏乳杆菌菌株具有较高的短期安全边际,这为其在畜牧业中的应用提供了充分的安全依据,但其长期、多代次使用的潜在生态安全风险仍是当前研究的空白领域,需深入探索。

2 罗伊氏乳杆菌生物学功能简介

罗伊氏乳杆菌作为一种广泛存在于人和动物肠道中的益生菌,具有多种重要的生物学功能,从而改善宿主的机体健康[9]。在肠道屏障方面,罗伊氏乳杆菌不仅能够增强肠上皮紧密连接蛋白的表达,还能够通过活化Wnt/β-连环蛋白(β-catenin)信号通路,促进肠道干细胞增殖和肠上皮细胞更新,从而维持肠黏膜屏障的完整性[21,25]。在肠道代谢方面,罗伊氏乳杆菌也发挥着重要作用,如促进短链脂肪酸(short chain fatty acids,SCFAs)合成[26]、改善胆汁酸代谢[27]和维持色氨酸代谢[28]等。在肠道稳态被破坏的情况下,如产肠毒素大肠杆菌(enterotoxigenic Escherichia coli,ETEC)攻毒和脂多糖(lipopolysaccharide,LPS)处理等,罗伊氏乳杆菌能够抑制促炎细胞因子的产生,调节辅助性T细胞1/辅助性T细胞2平衡,增加调节性T细胞比例,从而维持肠道免疫[29-30]。研究也发现,罗伊氏乳杆菌可直接通过分泌活性因子调控肠道激素,如分泌血清素、肽YY,进而影响肠道免疫[31]。在肠道微生物方面,罗伊氏乳杆菌能够有效抑制有害菌(如大肠杆菌、葡萄球菌等)生长并促进有益菌(如乳酸杆菌、芽孢杆菌和双歧杆菌等)增殖,从而发挥其益生作用[4,32]。值得注意的是,罗伊氏乳杆菌对肠道微生物群的调控能够影响肠道胆汁酸代谢,进而通过作用于胆汁酸受体来改善肠道健康[27]
此外,近年来许多研究揭示了罗伊氏乳杆菌代谢物与宿主互作的精确机制。例如,罗伊氏乳杆菌DYNDL22M62可调节肠道微生物组成,增强肠道色氨酸代谢,诱导芳香烃受体(aryl hydrocarbon receptor,AHR)配体吲哚乳酸和吲哚丙酸产量增加,从而激活AHR信号传导[33]。罗伊氏菌素会破坏细胞内的氧化还原平衡,导致细胞无法控制的活性氧产生,最终诱导细胞死亡,从而达到抗菌的效果[34]。罗伊氏乳杆菌分泌的细胞外囊泡(extracellular vesicles,EVs)同样是其与宿主互作的重要媒介,来自鸡源罗伊氏乳杆菌BBC3的EVs能够被巨噬细胞内化,并通过抑制核因子-κB(nuclear factor-κB,NF-κB)信号通路,显著下调促炎细胞因子的表达,同时上调抗炎细胞因子的水平,从而在急性炎症模型中有效重塑免疫平衡[35]。这些多层次的生物学功能使罗伊氏乳杆菌在预防肠道紊乱、维持肠道正常结构和功能等方面展现出重要应用价值。不过,罗伊氏乳杆菌的益生功效具有显著的菌株特异性,不同来源、不同分型的菌株在功能侧重和应用效果上存在差异。表1汇总了国内外研究中涉及的不同来源的罗伊氏乳杆菌菌株及其特性[11,14-15,20,32,36-43],以便更直观地进行比较和参考。
表1 不同来源的罗伊氏乳杆菌代表性菌株特性比较

Table 1 Comparison of characteristics of representative strains of Lactobacillus reuteri from different sources

菌株编号
Strain number
来源
Sources
试验模型/试验动物
Test model/
test animals
饲喂方式及剂量
Feeding methods
and dosages
功能特性
Functional
property
参考文献
References
LR1 仔猪 拌喂,
5×10¹⁰ CFU/kg
提高生长性能,改善小肠绒毛形态,提
高肠道紧密连接蛋白、黏液素、抗菌肽
及Toll样受体基因的表达,改善断奶
仔猪肠道上皮屏障功能
[20]
TPC32 藏猪
粪便
小鼠 灌胃,
1×10⁸ CFU/d
减少肠道病原菌的定植和减少肠
黏膜损伤,增强肠道免疫屏障
[11]
SLZX19-12 藏猪
粪便
小鼠 灌胃150 μL,
1×10⁹ CFU/mL
增强肠道微生物群的稳定性和屏障
完整性并减少炎症,从而保护
结肠免受感染
[36]
I5007 仔猪 母猪和仔猪 母猪拌喂,
1×10⁹ CFU/kg;
仔猪灌胃5 mL,
1×10⁹ CFU/mL
母猪:提高初乳中乳酸含量以及脐带
血血清中肿瘤坏死因子-α(TNF-α)和
白细胞介素-6(IL-6)含量;调节肠道
菌群,提高有益菌丰度,降低有
害菌丰度。仔猪:降低仔猪
血清IL-6含量
[32]
ZY15 小鼠 灌胃200 μL,
1×10⁹ CFU/mL
增强肠道微生物群稳定性和屏障
完整性,减少氧化应激引起的炎症来
保护回肠免受产肠毒素大肠杆菌
(ETEC)K88感染
[37]
RGW1 犊牛 小鼠 灌胃,
200 μL/d
(1×10⁸ CFU)
高疏水、对酸和胆汁盐耐受性强,
抗病原和免疫调节作用
[38]
L81 犊牛 犊牛 拌喂,2 g/d 有效改善犊牛断奶后肠道组织形态,
增强肠上皮屏障功能,缓解早期断奶
引起的应激反应和肠道损伤,增强
犊牛对断奶腹泻的抵抗力
[39]
SL001 白羽雏鸡 拌喂,
3×10⁸ CFU/g
促进肉鸡生长性能提高,增强
免疫力,改善抗氧化应激以及
肠道形态和微生物群落
[40]
22 拌喂,
1×10⁸ CFU/d
调节免疫,提高肠道中富含亮氨酸重复
序列G蛋白偶联受体5(Lrg5)、轴抑制
蛋白2(Axin2)和低密度脂蛋白受体
相关蛋白5(Lrp5)的mRNA表达,
激活Wnt/β-连环蛋白信号
通路诱导肠道增殖
[41]
KUB-AC5 小鼠巨噬细胞系
RAW264.7(ATCC
TIB-71)和人
膀胱上皮细胞系
UM-UC-3
黏附在人膀胱上皮上,减少尿路
致病性大肠杆菌(UPEC)菌株
黏附和人膀胱上皮的侵袭;通过
免疫调节增加巨噬细胞杀伤活性
[15]
PIA16 肉鸡雏鸡 拌喂,
1.89×10⁸ CFU/g
可增强鸡群免疫力,降低
死亡率,提高产量
[42]
FN041/DSM17938 小鼠 灌胃,
1×10⁹ CFU/d
调节免疫,降低血浆白细胞介
素-4(IL-4)、白细胞介素-33
(IL-33)含量;改善肠道菌群
[43]
FN041 小鼠 灌胃,
1×10⁹ CFU/d
促进后代肠道分泌型免疫球蛋
白A(sIgA)的产生和抗菌肽相关
基因的表达,增强黏膜屏障功能
[14]

3 罗伊氏乳杆菌在仔猪生产中的应用

在实际养猪生产中,罗伊氏乳杆菌作为一种有效的饲用益生菌,其应用需重点解决菌株活性保存、制剂稳定性及与饲粮兼容性等关键技术问题。为保障菌株长期存活,通常采用低温冷冻保存法或液氮超低温保存法;而在饲料添加剂生产中,则普遍通过真空冷冻干燥技术制备冻干粉,该工艺可有效去除水分并使菌体进入休眠状态,显著延长产品在室温下的保质期。此外,为进一步保护菌株免受胃酸和胆盐的侵蚀,提高肠道定植率,微胶囊包被技术已被广泛应用[44]。研究表明,微囊化罗伊氏乳杆菌LFCA能有效实现乳酸菌和抗菌肽的肠道靶向递送,并调节肠道微生物群和黏膜免疫[45]
在具体应用方案方面,综合现有研究,为预防仔猪断奶应激,多从断奶前几日开始添加,并持续至断奶后数周,以覆盖肠道微生物群建立和免疫系统发育的关键窗口期。罗伊氏乳杆菌在仔猪饲粮中的添加剂量多因菌株特性、制剂形式和饲养环境而异(表1)。综合多数研究,其在仔猪饲粮中的有效添加剂量通常为1×10⁸~1×10¹⁰ CFU/kg。与益生元联用(形成合生元)可产生协同效应,罗伊氏乳杆菌与低聚半乳糖组成的合生元可有效缓解肠道炎症和屏障功能障碍[19]。此外,复合益生菌制剂也是常见策略。例如,植物乳杆菌和罗伊氏乳杆菌可促进肠道健康,降低腹泻率,且两菌联合使用效果优于单一菌[46]。含有罗伊氏乳杆菌的7菌株复合制剂对仔猪生长性能的提升不显著,但该制剂仍能有效降低死亡率,并在免疫调节方面发挥作用[47]

3.1 提高仔猪增重

随着罗伊氏乳杆菌在畜牧业中的应用研究日益增多,其对动物生长性能的促进作用引起了广泛关注。在仔猪领域,多项研究评估了不同来源、分型的罗伊氏乳杆菌菌株对仔猪生长性能和死亡率的影响。此外,王琪等[46]研究显示,植物乳杆菌与罗伊氏乳杆菌联合使用可显著提高哺乳仔猪日增重,且效果优于单一菌种。Tang等[48]研究发现,含罗伊氏乳杆菌的复合制剂(与植物乳杆菌、长双歧杆菌联用)的饲粮通过改善肠道屏障和菌群结构,可促进仔猪平均日增重,减轻炎症反应和氧化应激。值得注意的是,罗伊氏乳杆菌提高仔猪增重可能与其调控氨基酸代谢的功能有关。He等[49]研究发现,罗伊氏乳杆菌LR1能够促进仔猪小肠中氨基酸转运蛋白溶质载体家族6成员19(SLC6A19)、溶质载体家族6成员9(SLC6A9)、溶质载体家族7成员1(SLC7A1)和溶质载体家族38成员9(SLC38A9)的表达,提高血清中甘氨酸和羟脯氨酸含量。
在降低死亡率方面,罗伊氏乳杆菌同样表现出积极效果。菌株KT260178可通过改善盲肠菌群和免疫功能降低仔猪发病率与死亡率[4];含罗伊氏乳杆菌的复合益生菌虽未显著提高增重,但能通过上调抗炎因子降低死亡率[47];其后生元制剂也可使断奶仔猪死亡率降低6.37%[26]。综上所述,罗伊氏乳杆菌在促进仔猪生长和降低死亡率方面展现出积极作用,支持其作为有效益生菌在畜牧业中应用。

3.2 减少仔猪腹泻

断奶后腹泻通常与肠道屏障紊乱有关,表现为肠道通透性增加,导致水分和电解质流失加剧,从而引发腹泻[50]。罗伊氏乳杆菌在减轻仔猪腹泻方面展现了显著的应用潜力。研究表明,腹泻仔猪肠道中的罗伊氏乳杆菌丰度显著降低[51]。在与添加植物乳杆菌CGMCC 1258的对比试验中,Tang等[52]发现,饲喂猪源罗伊氏乳杆菌LR1的断奶仔猪表现出更好的生长性能和更低的腹泻发生率。罗伊氏乳杆菌I5007能够调节肠道菌群结构,促进肠道健康,从而降低断奶仔猪腹泻率[46]。在养猪生产中,致病菌大肠杆菌(如ETEC)和沙门氏菌(如鼠伤寒沙门氏菌)是引发仔猪腹泻的主要病原体[53-54]。研究显示,罗伊氏乳杆菌能有效降低这些病原菌在肠道的负荷,减少其定植[55-56]。藏猪源罗伊氏乳杆菌F1菌株能够抑制沙门氏菌的生长[57]。菌株PF20-3和PF30-3对大肠杆菌和沙门氏菌具有直接抑菌活性[58]。综上所述,罗伊氏乳杆菌能够通过其直接和间接的抗菌、免疫调节及微生物调节作用,降低肠道病原体负荷,有效减轻仔猪腹泻。罗伊氏乳杆菌对仔猪生长性能的影响见表2[3-4,20,59-62]
表2 罗伊氏乳杆菌对仔猪生长性能的影响

Table 2 Effects of Lactobacillus reuteri on growth performance of piglets

试验对象
Experiment
objects
样本量
Sample
size
攻毒模型
Toxicity
model
菌株编号
Strain
number
饲喂时间
Feeding
time/d
饲喂方式及剂量
Feeding methods
and dosages
效果
Effects
参考文献
References
1日龄新生仔猪
One-day-old
newborn piglets
n=12头 猪传染性胃
肠炎病毒
(TGEV)
pPG-LFCA/
LR-CO21
7 灌胃,
2×10¹⁰ CFU/d
平均日增重↑,
腹泻和死亡率↓
[59]
1日龄新生仔猪
One-day-old
newborn piglets
n=3栏
(每栏9头)
I5007 10、20 灌胃,
1×10¹⁰ CFU/d
1~10日龄平均日
增重无显著差异;
11~20日龄平均
日增重↑,腹泻↓
[60]
1日龄新生仔猪
One-day-old
newborn piglets
n=20头 KT260178 28 拌喂,
1×10⁷ CFU/g
最终体重无显著
差异,死亡率和
发病率↓
[4]
21日龄断奶仔猪
Weaned piglets at
21 days of age
n=8栏
(每栏6头)
LR1 42 拌喂,
5×10¹⁰ CFU/kg
平均日增重↑ [20]
21日龄断奶仔猪
Weaned piglets at
21 days of age
n=6栏
(每栏4头)
IDCC 3701 28 拌喂,0.02% 平均日增重↑,
未显著缓解腹泻
[3]
28日龄断奶仔猪
Weaned piglets at
28 days of age
n=6栏
(每栏8头)
SLZX19-12 28 拌喂,
1.38×10⁸ CFU/kg
平均日增重↑,
腹泻↓
[61]
30日龄断奶仔猪
Weaned piglets at
30 days of age
n=5栏
(每栏5头)
PSC102 28 拌喂,
1×10⁹ CFU/g
生长速率和饲料
效率↑,腹泻↓
[62]

↑:提升 increase;↓:降低 decrease。

3.3 改善仔猪肠道屏障功能

健全的肠道屏障是仔猪抵御病原微生物入侵、维持肠道稳态和健康生长的关键基础[63]。肠道屏障由肠道黏液层、上皮细胞及其紧密连接、免疫细胞、共生微生物及其代谢产物等共同构成[64-65],肠道屏障功能受损会严重影响仔猪的生长发育,甚至导致死亡。罗伊氏乳杆菌可通过改善肠道形态结构来增强肠道屏障功能[39]。在仔猪空肠、回肠和十二指肠中,绒毛高度与隐窝深度比值(绒隐比)的升高,是反映肠道形态结构改善的直接指标[5,59]。刘春艳[20]发现,在断奶仔猪基础饲粮中添加罗伊氏乳杆菌LR1可显著提高十二指肠、空肠和回肠绒毛高度,并显著提高十二指肠和回肠绒隐比。紧密连接蛋白是维持肠道上皮物理屏障完整性的核心,罗伊氏乳杆菌能显著上调这些关键蛋白的表达;罗伊氏乳杆菌(如LR1、TPC32)能显著上调结肠和盲肠中闭锁小带蛋白-1(ZO-1)、闭合蛋白(Occludin)等关键紧密连接蛋白的表达,从而增强仔猪肠道屏障功能[20,66-67]
罗伊氏乳杆菌可通过调控关键信号通路缓解炎症,间接保护肠道屏障。Gao等[68]发现,在ETEC K88攻毒后,罗伊氏乳杆菌LR1通过抑制IPEC-J2细胞中肌球蛋白轻链激酶(myosin light-chain kinase,MLCK)信号通路活性降低炎症反应,从而改善肠上皮屏障功能;罗伊氏乳杆菌的有益代谢产物同样有助于屏障功能,例如罗伊氏乳杆菌发酵上清液被证实能够促进肠上皮细胞的生长和增殖,增强肠上皮细胞系Caco-2模型中的肠道屏障功能,这些作用在断奶仔猪模型中也得到了验证[69]。综上所述,罗伊氏乳杆菌通过多靶点机制(改善肠道结构、增强紧密连接、调节炎症/凋亡信号通路、产生有益代谢物SCFAs)综合提升仔猪肠道屏障功能,为仔猪健康生长提供重要保障。

3.4 调节仔猪肠道免疫,缓解肠道炎症

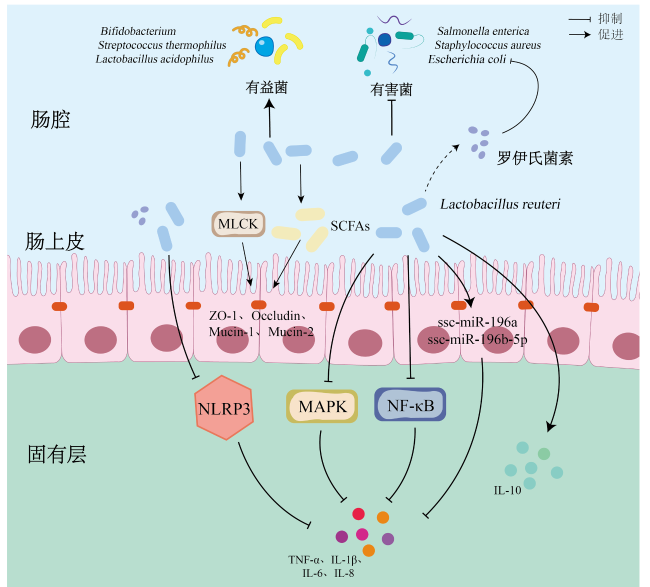
仔猪肠道炎症主要由于肠道发育不成熟及断奶应激所引发,进而导致免疫力下降和病原菌易感性增加[70]。研究显示,罗伊氏乳杆菌通过多途径调节仔猪肠道免疫,缓解肠道炎症(图1)。罗伊氏乳杆菌ZJ617通过介导肠道丝裂原活化蛋白激酶(mitogen-activated protein kinase,MAPK)和自噬信号通路,调节肠道内容物的代谢产物及其代谢途径,从而有效缓解LPS诱导的肠道炎症反应[71]。罗伊氏乳杆菌LR1能够减轻LPS导致的NOD样受体家族pyrin结构域包含蛋白3(NOD-like receptor family pyrin domain containing protein 3,NLRP3)炎症小体的激活,从而抑制促炎因子的表达[72]。微囊化罗伊氏乳杆菌LFCA菌株可抑制NF-κB和p38 MAPK信号通路,减轻沙门氏菌引起的仔猪肠黏膜炎症[45]。罗伊氏乳杆菌与牛奶L-谷氨酰胺的联用,还能抑制p38和c-Jun N端激酶(c-Jun N-terminal kinase,JNK)的磷酸化以及胱天蛋白酶(Caspase)3的激活,调节肠道菌群并缓解结肠炎症,改善仔猪肠道健康[73]。此外,罗伊氏乳杆菌LFCA可通过MLCK信号通路提升紧密连接蛋白[密封蛋白-1(Claudin-1)、Occludin、ZO-1]表达,并抑制NF-κB信号通路来增强抗炎效果,减少由肠致病性大肠杆菌感染引起的肠黏膜炎症因子和氧化应激的产生[74]
图1 罗伊氏乳杆菌改善仔猪肠道健康的作用机制

Bifidobacterium:双歧杆菌属;Streptococcus thermophilus:嗜热链球菌;Lactobacillus acidophilus:嗜酸乳杆菌;Salmonella enterica:肠炎沙门氏菌;Staphylococcus aureus:金黄色葡萄球菌;Escherichia coli:大肠杆菌;MLCK:肌球蛋白轻链激酶 myosin light-chain kinase;SCFAs:短链脂肪酸 short chain fatty acids;Lactobacillus reuteri:罗伊氏乳杆菌;ZO-1:闭锁小带蛋白-1 zonula occludens-1;Occludin:闭合蛋白;Mucin:黏蛋白;NLRP3:NOD样受体家族pyrin结构域包含蛋白3 NOD-like receptor family pyrin domain containing protein 3;MAPK:丝裂原活化蛋白激酶 mitogen-activated protein kinase;IL-10:白细胞介素-10 interleukin-10;TNF-α:肿瘤坏死因子-α tumor necrosis factor-α;IL-1β:白细胞介素-1β interleukin-1β;IL-6:白细胞介素-6 interleukin-6;IL-8:白细胞介素-8 interleukin-8。

Fig.1 Mechanism by which Lactobacillus reuteri improved intestinal health of piglets[4,6,45,56,69-76]

值得注意的是,罗伊氏乳杆菌对肠道炎症的调控可能受到更上游表观遗传影响。研究发现,罗伊氏乳杆菌I5007处理可通过改变回肠微小RNA(miRNA)表达谱来调节肠道免疫,该研究鉴定出19个差异表达的miRNA,其靶基因显著富集于磷脂酰肌醇3-激酶(PI3K)-蛋白激酶B(Akt)和MAPK等关键信号通路;更重要的是,研究发现罗伊氏乳杆菌I5007处理后高表达的ssc-miR-196a和ssc-miR-196b-5p可下调IPEC-J2细胞中白细胞介素-1β(IL-1β)和肿瘤坏死因子-α(TNF-α)的mRNA表达,有效缓解炎症[75]。在仔猪活体水平,罗伊氏乳杆菌能够有效抑制促炎因子,如白细胞介素-6(IL-6)、白细胞介素-8(IL-8)和TNF-α在空肠和结肠的表达,并且能够上调抗炎因子白细胞介素-10(IL-10)在回肠和结肠中的表达[5,76]。综上所述,罗伊氏乳杆菌通过多途径有效缓解仔猪肠道炎症,共同维护肠道免疫稳态,为仔猪健康生长奠定基础。

3.5 重塑仔猪肠道菌群结构与功能

肠道菌群稳态是维持仔猪肠道正常生理功能的基础,其失调可引发炎症反应、氧化应激等不良后果[77]。因此,肠道菌群稳态的调控已成为改善仔猪肠道健康的核心策略。罗伊氏乳杆菌作为重要益生菌,其核心功能之一便是有效重塑紊乱的肠道微生物群落结构,从而维护肠道完整性、增强屏障功能,并最终改善整体肠道健康[36,78]
在仔猪生产中,罗伊氏乳杆菌可显著提升肠道内有益菌丰度,降低有害菌丰度,从而调节肠道菌群结构(图1)。研究发现,饲粮添加罗伊氏乳杆菌KT260178能够有效促进盲肠微生物群落的稳定性,增强盲肠中乳杆菌属和双歧杆菌属丰度,并且降低大肠杆菌属和葡萄球菌属数量[4]。饲粮添加罗伊氏乳杆菌ZLR003可显著提升猪肠道中拟杆菌属、乳杆菌属和双歧杆菌属丰度,同时抑制潜在致病菌的丰度[6]。值得注意的是,母体饲喂罗伊氏乳杆菌可通过影响初乳中的微生物群落,减少有害细菌(如变形菌门)并增加有益细菌(如绒毛膜双歧杆菌),同时调整初乳的功能成分,从而促进仔猪肠道微生物群落的发育[32]。针对仔猪生产中最常见的致病菌ETEC,研究发现,罗伊氏乳杆菌能够有效抑制大肠杆菌F18ac黏附在猪IPEC-J2细胞上[54]。此外,罗伊氏乳杆菌LR1的代谢产物罗伊氏菌素在体外能够有效抑制ETEC K88生长,进一步证明了罗伊氏乳杆菌对肠道微生物稳态的保护作用[18]。这些结果表明,罗伊氏乳杆菌对仔猪肠道健康具有积极影响,能够调节肠道微生物稳态来改善肠道健康并促进仔猪健康生长。

4 小结与展望

罗伊氏乳杆菌凭借其丰富的菌株资源和卓越的益生特性,在促进仔猪生长性能、改善肠道健康方面发挥着重要作用,是替代抗生素的有力候选者。然而,其广泛应用仍面临挑战,未来的研究应聚焦于关键领域。深入评估其长期使用的安全性,特别是抗生素耐药基因通过水平转移在微生物群落中扩散的潜在生态风险;系统解析罗伊氏乳杆菌与复杂饲粮体系中其他组分(如矿物质、有机酸)的互作机制,以明确其在实际生产中的真实效价;还可借鉴食品科学等领域的先进技术(如制剂包埋与工艺优化),开发新一代高效、稳定的产品。解决这些核心问题,将为罗伊氏乳杆菌在畜牧业中的安全、高效应用提供坚实保障,从而有力推动无抗养殖的可持续发展。
[1]
KECHAGIA M, BASOULIS D, KONSTANTOPOULOU S, et al. Health benefits of probiotics:a review[J]. International Scholarly Research Notices, 2013, 2013(1):481651.

[2]
GIRAFFA G, CHANISHVILI N, WIDYASTUTI Y. Importance of Lactobacilli in food and feed biotechnology[J]. Research in Microbiology, 2010, 161(6):480-487.

DOI

[3]
KANG Y G, KYOUNG H, PARK K I, et al. PSXIII-10 effects of dietary Lactobacillus reuteri on growth performance,frequency of diarrhea,and blood biochemical parameters of weaned pigs[J]. Journal of Animal Science, 2023, 101(S3):576-577.

DOI

[4]
YANG J J, WANG C L, LIU L Q, et al. Lactobacillus reuteri KT260178 supplementation reduced morbidity of piglets through its targeted colonization,improvement of cecal microbiota profile,and immune functions[J]. Probiotics and Antimicrobial Proteins, 2020, 12(1):194-203.

DOI

[5]
XIE Q, YANG M, DUANMU Q, et al. Ningxiang pig-derived Lactobacillus reuteri improves the gut health of weaned piglets by regulating intestinal barrier function and cytokine profiles[J]. Scientific Reports, 2025, 15(1):3993.

DOI

[6]
ZHANG D Y, WANG S X, LI G X, et al. Two doses of Lactobacillus induced different microbiota profiles and serum immune indices in pigs[J]. Journal of Functional Foods, 2023, 102:105405.

DOI

[7]
HA S, KYOUNG H, PARK K I, et al. PSXIII-8 effects of dietary Lactobacillus reuteri on immune responses,blood profiles,intestinal morphology,and ileal gene expression of weaned pigs[J]. Journal of Animal Science, 2023, 101(Suppl.3):569-570.

DOI

[8]
JIANG J Y, LI K, XIAO Y, et al. Limosilactobacillus reuteri regulating intestinal function:a review[J]. Fermentation, 2023, 9(1):19.

DOI

[9]
YU Z H, CHEN J H, LIU Y X, et al. The role of potential probiotic strains Lactobacillus reuteri in various intestinal diseases:new roles for an old player[J]. Frontiers in Microbiology, 2023, 14:1095555.

DOI

[10]
MU Q H, TAVELLA V J, LUO X M. Role of Lactobacillus reuteri in human health and diseases[J]. Frontiers in Microbiology, 2018, 9:757.

DOI

[11]
KONG Q H, SHANG Z D, NAWAZ S, et al. The whole-genome sequencing and probiotic profiling of Lactobacillus reuteri strain TPC32 isolated from Tibetan pig[J]. Nutrients, 2024, 16(12):1900.

DOI

[12]
UEZEN J D, FICOSECO C A, FÁTIMA NADER-MACÍAS M E, et al. Identification and characterization of potential probiotic lactic acid bacteria isolated from pig feces at various production stages[J]. Canadian Journal of Veterinary Research, 2023, 87(2):127-145.

[13]
LIU Z Z, ZHAO X, BANGASH H I, et al. Expression of stress responsive genes enables Limosilactobacillus reuteri to cross-protection against acid,bile salt,and freeze-drying[J]. Frontiers in Microbiology, 2024, 15:1437803.

DOI

[14]
QI C, DING M F, LI S Q, et al. Sex-dependent modulation of immune development in mice by secretory IgA-coated Lactobacillus reuteri isolated from breast milk[J]. Journal of Dairy Science, 2021, 104(4):3863-3875.

DOI

[15]
TANTIBHADRASAPA A, LI S B, BUDDHASIRI S, et al. Probiotic Limosilactobacillus reuteri KUB-AC5 decreases urothelial cell invasion and enhances macrophage killing of uropathogenic Escherichia coli in vitro study[J]. Frontiers in Cellular and Infection Microbiology, 2024, 14:1401462.

DOI

[16]
WANG D J, ZENG J Y, WUJIN C M, et al. Lactobacillus reuteri derived from horse alleviates Escherichia coli-induced diarrhea by modulating gut microbiota[J]. Microbial Pathogenesis, 2024, 188:106541.

DOI

[17]
李元元, 梁伟, 陈龙, 等. 牛源罗伊氏乳杆菌对产肠毒素大肠杆菌攻毒小鼠生长性能、免疫性能、抗氧化能力及肠道健康的影响[J]. 动物营养学报, 2024, 36(10):6768-6779.

DOI

LI Y Y, LIANG W, CHEN L, et al. Effects of Lactobacillus reuteri from cattle on growth performance,immune performance,antioxidant capacity and intestinal health of mice challenged with enterotoxigenic Escherichia coli[J]. Chinese Journal of Animal Nutrition, 2024, 36(10):6768-6779. (in Chinese)

[18]
吴奇, 杨希. 罗伊氏菌素对猪肠上皮细胞免疫调控研究及其在仔猪健康中的潜在应用[J]. 广东畜牧兽医科技, 2025, 50(3):53-62.

DOI

WU Q, YANG X. Study on the immune regulation of porcine intestinal epithelial cells by reuterin and its potential application in piglet health[J]. Guangdong Journal of Animal and Veterinary Science, 2025, 50(3):53-62. (in Chinese)

[19]
WU Y J, ZHANG X Y, LIU X Y, et al. Galactooligosaccharides and Limosilactobacillus reuteri synergistically alleviate gut inflammation and barrier dysfunction by enriching Bacteroides acidifaciens for pentadecanoic acid biosynthesis[J]. Nature Communications, 2024, 15(1):9291.

DOI

[20]
刘春艳. 猪源罗伊氏乳杆菌对断奶仔猪肠道屏障功能和细胞外基质的影响[D].硕士学位论文. 南宁: 广西大学, 2023.

LIU C Y. Effects of Lactobacillus reuteri from pigs on intestinal barrier function and extracellular matrix of weaned piglets[D].Master’s Thesis. Nanning: Guangxi University, 2023. (in Chinese)

[21]
DING X Q, TANG R Z, ZHAO J Y, et al. Lactobacillus reuteri alleviates LPS-induced intestinal mucosal damage by stimulating the expansion of intestinal stem cells via activation of the Wnt/β-catenin signaling pathway in broilers[J]. Poultry Science, 2024, 103(10):104072.

DOI

[22]
EFSA Panel on Biological Hazards (BIOHAZ),KOUTSOUMANIS K, ALLENDE A, et al. Update of the list of qualified presumption of safety (QPS) recommended microorganisms intentionally added to food or feed as notified to EFSA[J]. EFSA Journal, 2023, 21(1):e07747.

[23]
MANGALAT N, LIU Y Y, FATHEREE N Y, et al. Safety and tolerability of Lactobacillus reuteri DSM 17938 and effects on biomarkers in healthy adults:results from a randomized masked trial[J]. PLoS One, 2012, 7(9):e43910.

DOI

[24]
SENDELIUS M, AXELSSON J, LIU P D, et al. Genomic,phenotypic,and clinical safety of Limosilactobacillus reuteri ATCC PTA 4659[J]. Journal of Industrial Microbiology & Biotechnology, 2023, 50(1):kuad041.

[25]
WU H Q, XIE S, MIAO J F, et al. Lactobacillus reuteri maintains intestinal epithelial regeneration and repairs damaged intestinal mucosa[J]. Gut Microbes, 2020, 11(4):997-1014.

DOI

[26]
SUN D F, TONG W F, HAN S C, et al. Effects of dietary supplementation with Lactobacillus reuteri postbiotics on growth performance,intestinal flora structure and plasma metabolome of weaned piglets[J]. Animals, 2025, 15(2):204.

DOI

[27]
LIN Z S, WU J M, WANG J P, et al. Dietary Lactobacillus reuteri prevent from inflammation mediated apoptosis of liver via improving intestinal microbiota and bile acid metabolism[J]. Food Chemistry, 2023, 404(Pt B):134643.

[28]
LIU Z Y, LING Y D, PENG Y, et al. Regulation of serotonin production by specific microbes from piglet gut[J]. Journal of Animal Science and Biotechnology, 2023, 14(1):111.

DOI PMID

[29]
KIŠŠOVÁ Z, MUDROÑOVÁ D, LINK R, et al. Immunomodulatory effect of probiotic exopolysaccharides in a porcine in vitro co-culture model mimicking the intestinal environment on ETEC infection[J]. Veterinary Research Communications, 2024, 48(2):705-724.

DOI

[30]
XIE W C, WANG X Y, CAI J Y, et al. Optimum fermentation conditions for bovine lactoferricin-lactoferrampin-encoding Limosilactobacillus reuteri and regulation of intestinal inflammation[J]. Foods, 2023, 12(22):4068.

DOI

[31]
DI RIENZI S C, DANHOF H A, FORSHEE M D, et al. Limosilactobacillus reuteri promotes the expression and secretion of enteroendocrine- and enterocyte-derived hormones[J]. The FASEB Journal, 2025, 39(6):e70408.

DOI

[32]
WANG G, WANG X Y, MA Y H, et al. Lactobacillus reuteri improves the development and maturation of fecal microbiota in piglets through mother-to-infant microbe and metabolite vertical transmission[J]. Microbiome, 2022, 10(1):211.

DOI

[33]
FANG Z F, PAN T, WANG H C, et al. Limosilactobacillus reuteri attenuates atopic dermatitis via changes in gut bacteria and indole derivatives from tryptophan metabolism[J]. International Journal of Molecular Sciences, 2022, 23(14):7735.

DOI

[34]
LI J Y, WANG T, YANG X, et al. Systematic analysis of the antibacterial mechanisms of reuterin using the E.coli Keio collection[J]. mBio, 2025, 16(8):e0143225.

DOI

[35]
HU R J, LIN H, WANG M M, et al. Lactobacillus reuteri-derived extracellular vesicles maintain intestinal immune homeostasis against lipopolysaccharide-induced inflammatory responses in broilers[J]. Journal of Animal Science and Biotechnology, 2021, 12(1):25.

DOI

[36]
WU J M, LIN Z S, WANG X, et al. Limosilactobacillus reuteri SLZX19-12 protects the colon from infection by enhancing stability of the gut microbiota and barrier integrity and reducing inflammation[J]. Microbiology Spectrum, 2022, 10(3):e0212421.

DOI

[37]
XU X, ZHANG H W, MENG K, et al. Limosilactobacillus reuteri ZY15 alleviates intestinal inflammation and barrier dysfunction via AKT/mTOR/HIF-1α/RORγt/IL-17 signaling and the gut microbiota in ETEC K88-challenged mice[J]. Antioxidants, 2025, 14(1):58.

DOI

[38]
HUANG K L, SHI W B, YANG B, et al. The probiotic and immunomodulation effects of Limosilactobacillus reuteri RGW1 isolated from calf feces[J]. Frontiers in Cellular and Infection Microbiology, 2023, 12:1086861.

DOI

[39]
LI Y Y, LI X, NIE C X, et al. Effects of two strains of Lactobacillus isolated from the feces of calves after fecal microbiota transplantation on growth performance,immune capacity,and intestinal barrier function of weaned calves[J]. Frontiers in Microbiology, 2023, 14:1249628.

DOI

[40]
CHAI C L, GUO Y W, MOHAMED T, et al. Dietary Lactobacillus reuteri SL001 improves growth performance,health-related parameters,intestinal morphology and microbiota of broiler chickens[J]. Animals, 2023, 13(10):1690.

DOI

[41]
XIE S, ZHAO S Y, JIANG L, et al. Lactobacillus reuteri stimulates intestinal epithelial proliferation and induces differentiation into goblet cells in young chickens[J]. Journal of Agricultural and Food Chemistry, 2019, 67(49):13758-13766.

DOI

[42]
GONMEI G, SAPCOTA D, SAIKIA G K, et al. Studies on immune response to Newcastle disease virus in broiler chickens fed with Lactobacillus reuteri PIA16 isolated from the gut of indigenous chicken of Assam,India[J]. Veterinary World, 2019, 12(8):1251-1255.

DOI

[43]
ZHOU J B, XU G S, LI X Y, et al. Limosilactobacillus reuteri FN041 prevents atopic dermatitis in pup mice by remodeling the ileal microbiota and regulating gene expression in Peyer’s patches after vertical transmission[J]. Frontiers in Nutrition, 2022, 9:987400.

DOI

[44]
WANG X Y, XIE W C, ZHANG S H, et al. Effect of microencapsulation techniques on the stress resistance and biological activity of bovine lactoferricin-lactoferrampin-encoding Lactobacillus reuteri[J]. Foods, 2022, 11(20):3169.

DOI

[45]
WANG X Y, XIE W C, CAI L M, et al. Microencapsulated Limosilactobacillus reuteri encoding lactoferricin-lactoferrampin targeted intestine against Salmonella typhimurium infection[J]. Nutrients, 2023, 15(24):5141.

DOI

[46]
王琪, 肖融, 齐仁立, 等. 植物乳杆菌和罗伊氏乳杆菌对哺乳仔猪生长性能、肠道功能和盲肠菌群的影响[J]. 动物营养学报, 2024, 36(12):7658-7668.

DOI

WANG Q, XIAO R, QI R L, et al. Effects of Lactobacillus plantarum and Lactobacillus reuteri on growth performance,intestinal function and cecal microbiota of suckling piglets[J]. Chinese Journal of Animal Nutrition, 2024, 36(12):7658-7668. (in Chinese)

DOI

[47]
SAHATSANON K, SIVAPIRUNTHEP P, SRINGARM K, et al. Influence of host-specific and locally isolated multi-strain probiotics on piglet performance,mortality,inflammatory response,and gut microbiome[J]. Animal Bioscience, 2025, 38(4):717-727.

DOI

[48]
TANG J L, ZHAO M C, YANG W Y, et al. Effect of composite probiotics on antioxidant capacity,gut barrier functions,and fecal microbiome of weaned piglets and sows[J]. Animals, 2024, 14(9):1359.

DOI

[49]
HE Y Y, WEI Y Y, RUAN S H, et al. Dietary supplementation of Lactobacillus reuteri modulates amino acid metabolism and extracellular matrix in the gut-liver axis of weaned piglets[J]. Animals, 2025, 15(11):1567.

DOI

[50]
MCLAMB B L, GIBSON A J, OVERMAN E L, et al. Early weaning stress in pigs impairs innate mucosal immune responses to enterotoxigenic E.coli challenge and exacerbates intestinal injury and clinical disease[J]. PLoS One, 2013, 8(4):e59838.

DOI

[51]
ZHANG J Q, CHEN Y H, GUO X, et al. The gut microbial metabolite indole-3-aldehyde alleviates impaired intestinal development by promoting intestinal stem cell expansion in weaned piglets[J]. Journal of Animal Science and Biotechnology, 2024, 15(1):150.

DOI PMID

[52]
TANG Q S, YI H B, HONG W B, et al. Comparative effects of L.plantarum CGMCC 1258 and L.reuteri LR1 on growth performance,antioxidant function,and intestinal immunity in weaned pigs[J]. Frontiers in Veterinary Science, 2021, 8:728849.

DOI

[53]
SONG D, LEE J, KIM K, et al. Effects of dietary supplementation of Pediococcus pentosaceus strains from kimchi in weaned piglet challenged with Escherichia coli and Salmonella enterica[J]. Journal of Animal Science and Technology, 2023, 65(3):611-626.

DOI

[54]
QIN W Y, XIE Y X, REN Z S, et al. Integrative ATAC-seq and RNA-seq analyses of IPEC-J2 cells reveals porcine transcription and chromatin accessibility changes associated with Escherichia coli F18ac inhibited by Lactobacillus reuteri[J]. Frontiers in Microbiology, 2023, 14:1101111.

DOI

[55]
QIN W Y, REN Z S, XU C, et al. Chromatin accessibility and transcriptional landscape during inhibition of Salmonella enterica by Lactobacillus reuteri in IPEC-J2 cells[J]. Cells, 2023, 12(6):968.

DOI

[56]
ALI M S, LEE E B, LIM S K, et al. Isolation and identification of Limosilactobacillus reuteri PSC102 and evaluation of its potential probiotic,antioxidant,and antibacterial properties[J]. Antioxidants, 2023, 12(2):238.

DOI

[57]
CHANG Z Y, XIAO Q Q, YE Y R, et al. Isolation,identification and biological characteristics of Lactobacillus reuteri from Tibetan pigs[J]. Pakistan Journal of Zoology, 2024, 56(4):1757-1762.

[58]
YOO Y, LEE J, CHO J, et al. Antimicrobial properties of Limosilactobacillus reuteri strains for control of Escherichia coli and Salmonella strains,diarrhoea cause in weaning pigs[J]. Veterinarni Medicina, 2023, 68(5):191-199.

DOI

[59]
汪昭睿, 王雪莹, 解伟纯, 等. 重组猪源罗伊氏乳酸杆菌分泌表达牛乳铁蛋白肽对新生仔猪生长性能的影响以及抗腹泻病毒感染的保护作用研究[J]. 动物营养学报, 2022, 34(1):159-176.

DOI

WANG Z R, WANG X Y, XIE W C, et al. Effects of recombinant porcine Lactobacillus reuteri secreting expression of bovine lactoferrin peptides on growth performance of newborn piglets and protective effect against diarrhea virus infection[J]. Chinese Journal of Animal Nutrition, 2022, 34(1):159-176. (in Chinese)

[60]
WANG Q, WANG J, QI R L, et al. Effect of oral administration of Limosilactobacillus reuteri on intestinal barrier function and mucosal immunity of suckling piglets[J]. Italian Journal of Animal Science, 2022, 21(1):612-623.

DOI

[61]
WU J M, LIN Z S, WANG J P, et al. Limosilactobacillus reuteri alleviates weaned stress by improving immune function and gut microbiota in piglets[J]. Journal of Functional Foods, 2024, 114:106094.

DOI

[62]
CHO H Y, LEE G Y, ALI M S, et al. Effects of dietary intake of heat-inactivated Limosilactobacillus reuteri PSC102 on the growth performance,immune response,and gut microbiota in weaned piglets[J]. Pakistan Veterinary Journal, 2024, 44(3):819-825.

[63]
TAKIISHI T, FENERO C I M, CÂMARA N O S. Intestinal barrier and gut microbiota:shaping our immune responses throughout life[J]. Tissue Barriers, 2017, 5(4):e1373208.

DOI

[64]
HAN X B, HU X D, JIN W, et al. Dietary nutrition,intestinal microbiota dysbiosis and post-weaning diarrhea in piglets[J]. Animal Nutrition, 2024, 17:188-207.

DOI

[65]
TANG X P, XIONG K N. Dietary epidermal growth factor supplementation alleviates intestinal injury in piglets with intrauterine growth retardation via reducing oxidative stress and enhancing intestinal glucose transport and barrier function[J]. Animals, 2022, 12(17):2245.

DOI

[66]
YANG B J, LIU C Y, HUANG Y N, et al. The responses of Lactobacillus reuteri LR1 or antibiotic on intestinal barrier function and microbiota in the cecum of pigs[J]. Frontiers in Microbiology, 2022, 13:877297.

DOI

[67]
孔庆辉. 罗伊氏乳杆菌TPC32对LPS诱导断奶藏仔猪肠道损伤的保护作用研究[D].博士学位论文. 武汉: 华中农业大学, 2024:145.

KONG Q H. Protective effect of Lactobacillus reuteri TPC32 on LPS induced intestinal injury in Tibetan weaned piglets[D].Ph.D.Thesis. Wuhan: Huazhong Agricultural University, 2024:145. (in Chinese)

[68]
GAO J C, CAO S T, XIAO H, et al. Lactobacillus reuteri 1 enhances intestinal epithelial barrier function and alleviates the inflammatory response induced by enterotoxigenic Escherichia coli K88 via suppressing the MLCK signaling pathway in IPEC-J2 cells[J]. Frontiers in Immunology, 2022, 13:897395.

DOI

[69]
ABREHAME S, HUNG M Y, CHEN Y Y, et al. Selection of fermentation supernatant from probiotic strains exhibiting intestinal epithelial barrier protective ability and evaluation of their effects on colitis mouse and weaned piglet models[J]. Nutrients, 2024, 16(8):1138.

DOI

[70]
JIANG Z P, YANG M Z, SU W F, et al. Probiotics in piglet:from gut health to pathogen defense mechanisms[J]. Frontiers in Immunology, 2024, 15:1468873.

DOI

[71]
朱涛. 罗伊氏乳杆菌ZJ617对LPS致炎仔猪肠道和肝脏的保护效应及机制研究[D].硕士学位论文. 杭州: 浙江大学, 2021.

ZHU T. Protective effect and mechanism of Lactobacillus reuteri ZJ617 on intestine and liver of piglets induced by lipopolysaccharides[D].Master’s Thesis. Hangzhou: Zhejiang University, 2021. (in Chinese)

[72]
高靖春. 罗伊氏乳杆菌 (LR1) 对仔猪肠黏膜屏障功能的影响[D].硕士学位论文. 广州: 仲恺农业工程学院, 2023.

GAO J C. Effect of Lactobacillus reuteri (LR1) on intestinal mucosal barrier function in piglets[D].Master’s Thesis. Guangzhou: Zhongkai University of Agriculture and Engineering, 2023. (in Chinese)

[73]
WANG C, WEI S Y, LIU B J, et al. Maternal consumption of a fermented diet protects offspring against intestinal inflammation by regulating the gut microbiota[J]. Gut Microbes, 2022, 14(1):2057779.

DOI

[74]
XIE W C, SONG L Y, WANG X Y, et al. A bovine lactoferricin-lactoferrampin-encoding Lactobacillus reuteri CO21 regulates the intestinal mucosal immunity and enhances the protection of piglets against enterotoxigenic Escherichia coli K88 challenge[J]. Gut Microbes, 2021, 13(1):1956281.

DOI

[75]
WANG Q, SUN Q, WANG J, et al. Identification of differentially expressed miRNAs after Lactobacillus reuteri treatment in the ileum mucosa of piglets[J]. Genes & Genomics, 2020, 42(11):1327-1338.

[76]
ZHU Y B, CAI H M, YAN Z Q, et al. Alleviating Pentatrichomonas hominis-induced damage in IPEC-J2 cells:the beneficial influence of porcine-derived Lactobacilli[J]. Veterinary Research Communications, 2024, 48(4):2331-2342.

DOI

[77]
HE Y, WANG S H, LU H N, et al. Imbalance of intestinal flora activates inflammatory response contributing to acute lung injury[J]. Journal of Thoracic Disease, 2024, 16(10):6835-6848.

DOI PMID

[78]
SHEN J, WANG S T, HUANG Y, et al. Lactobacillus reuteri ameliorates lipopolysaccharide-induced acute lung injury by modulating the gut microbiota in mice[J]. Nutrients, 2023, 15(19):4256.

DOI

Outlines

/