RESEARCH PAPER

Effects of Tryptophan on Intestinal and Testicular Injury Induced by Deoxynivalenol in Mice

  • ZHANG Le ,
  • ZHANG Ruinan ,
  • WU Yihan ,
  • WU De ,
  • LIN Yan ,
  • FENG Bin ,
  • ZHUO Yong ,
  • CHE Lianqiang ,
  • XU Shengyu ,
  • HUA Lun ,
  • FANG Zhengfeng ,
  • JIANG Xuemei ,
  • LI Jian ,
  • LIU Guangmang , **
Expand
  • Key Laboratory of Animal Disease-Resistant Nutrition, Ministry of Education, Institute of Animal Nutrition, Sichuan Agricultural University, Chengdu 611130, China
**associate professor, E-mail:

*Contributed equally

Received date: 2025-09-16

  Online published: 2026-04-14

Abstract

This experiment was conducted to explore the effects of tryptophan on intestinal and testicular injury induced by deoxynivalenol (DON) in mice. Forty-eight 7-week-old specific pathogen free (SPF) male C57BL/6 mice were selected and randomly divided into 4 groups, with 12 replicates in each group and 1 mouse in each replicate. Mice in each group were fed the same basal diet. Meanwhile, the control group (CON group) was gavaged with alanine (equal nitrogen to tryptophan, the same as below), the tryptophan group (TRP group) was gavaged with 150 mg/kg BW tryptophan, the DON group was gavaged with 2.0 mg/kg BW DON and alanine, and the DON+tryptophan group (DON+TRP group) was gavaged with 2.0 mg/kg BW DON+150 mg/kg BW tryptophan. The experiment lasted for 21 days. The results showed as follows: 1) compared with the CON group, the final body weight of mice in the DON group was significantly decreased (P<0.05), and DON caused injury to the jejunum and testis. 2) Compared with the DON group, the activities of catalase, glutathione peroxidase and total superoxide dismutase as well as glutathione content in jejunum in the DON+TRP group were significantly increased (P<0.05), while the malondialdehyde content in jejunum was significantly decreased (P<0.05); the jejunal crypt depth and the serum diamine oxidase activity in the DON+TRP group were significantly decreased (P<0.05), while the villus height to crypt depth ratio and the occludin content in jejunum were significantly increased (P<0.05); the spermatogenic tubule diameter and epithelium thickness of testis were significantly increased (P<0.05), and the serum testosterone content and sperm motility were significantly increased (P<0.05). In conclusion, tryptophan can alleviate the intestinal and testicular injury induced by DON in mice by enhancing the antioxidant capacity of jejunum, improving the morphology and barrier function of jejunum, improving the testicular morphology, and increasing the serum testosterone content and sperm motility.

Cite this article

ZHANG Le , ZHANG Ruinan , WU Yihan , WU De , LIN Yan , FENG Bin , ZHUO Yong , CHE Lianqiang , XU Shengyu , HUA Lun , FANG Zhengfeng , JIANG Xuemei , LI Jian , LIU Guangmang . Effects of Tryptophan on Intestinal and Testicular Injury Induced by Deoxynivalenol in Mice[J]. Chinese Journal of Animal Nutrition, 2026 , 38(4) : 3058 -3065 . DOI: 10.12418/CJAN2026.245

脱氧雪腐镰刀菌烯醇(DON,又称呕吐毒素)是一种常存在于小麦、玉米等农作物中的霉菌毒素[1],其毒性主要源于C9~C10双键、C12~C13环氧基和C3羟基[2]。DON的靶器官主要是肠道,其主要被胃肠道吸收和代谢,部分可分布到其他组织,导致器官损伤[3]。DON可降低动物肠道绒毛高度和紧密连接蛋白表达,诱导氧化应激,提高隐窝深度和促炎因子含量[4-6]。这揭示DON可诱导肠道炎症,损害肠道结构和功能完整性。DON还可造成线粒体功能障碍、内质网应激和炎症反应等,导致机体肝脏毒性和生殖毒性[7-8]。研究表明,口服灌胃2.0 mg/kg BW DON降低小鼠体重和血清睾酮含量,造成睾丸损伤[9]。DON降低小鼠曲细精管直径、生精上皮厚度、精子密度和精子活力[8,10]。色氨酸能调控促炎和抗炎细胞因子含量,缓解氧化应激,促进肠道健康[11]。色氨酸代谢产物褪黑素能提高精液品质,5-羟色胺能促进精子的顶体反应,这说明色氨酸与雄性繁殖可能有重要的联系[12-13]。然而,目前尚缺乏色氨酸缓解DON诱导的动物肠道和睾丸损伤的研究,本研究旨在探究色氨酸是否能够缓解DON诱导的小鼠肠道和睾丸损伤。

1 材料与方法

1.1 试验设计

本试验方案已通过四川农业大学实验动物伦理委员会审批(批准编号:SICAU-2024-12)。试验小鼠饲粮由成都达硕实验动物有限公司提供。饲粮主要营养成分含量及测定所参考的国标方法如下:水分9.5%(GB/T 6435—2014)、粗蛋白质20.5%(GB/T 6432—2018)、粗脂肪5.6%(GB/T 6433—2006)、粗纤维3.3%(GB/T 6434—2006)、粗灰分6.8%(GB/T 6438—2007)、钙1.27%(GB/T 6436—2018)和磷0.85%(GB/T 6437—2018)。
试验选用48只7周龄无特定病原体(SPF)级雄性C57BL/6小鼠(体重18~20 g,购自成都达硕实验动物有限公司),饲养环境条件为温度(23±2) ℃、相对湿度50%~60%、12 h昼夜光照,自由摄食和饮水。试验小鼠在四川农业大学实验房预试1周后,随机分为4组,分别为对照组(CON组)、色氨酸组(TRP组)、DON组和DON+色氨酸组(DON+TRP组),每组12个重复,每个重复1只。所有小鼠饲喂基础饲粮(SPF繁殖料),并分别给予灌胃丙氨酸(S20001-500 g,与色氨酸等氮,后同)、色氨酸(150 mg/kg BW,L-色氨酸:S20082-500 g)[14]、DON(2.0 mg/kg BW)[3]和丙氨酸混合液以及DON(2.0 mg/kg BW)+色氨酸(150 mg/kg BW)混合液,连续21 d(图1-A)。试验结束后,收集所有试验小鼠血清样本;并取部分空肠和睾丸组织固定于4%多聚甲醛溶液,其余冻存于-80 ℃待用。
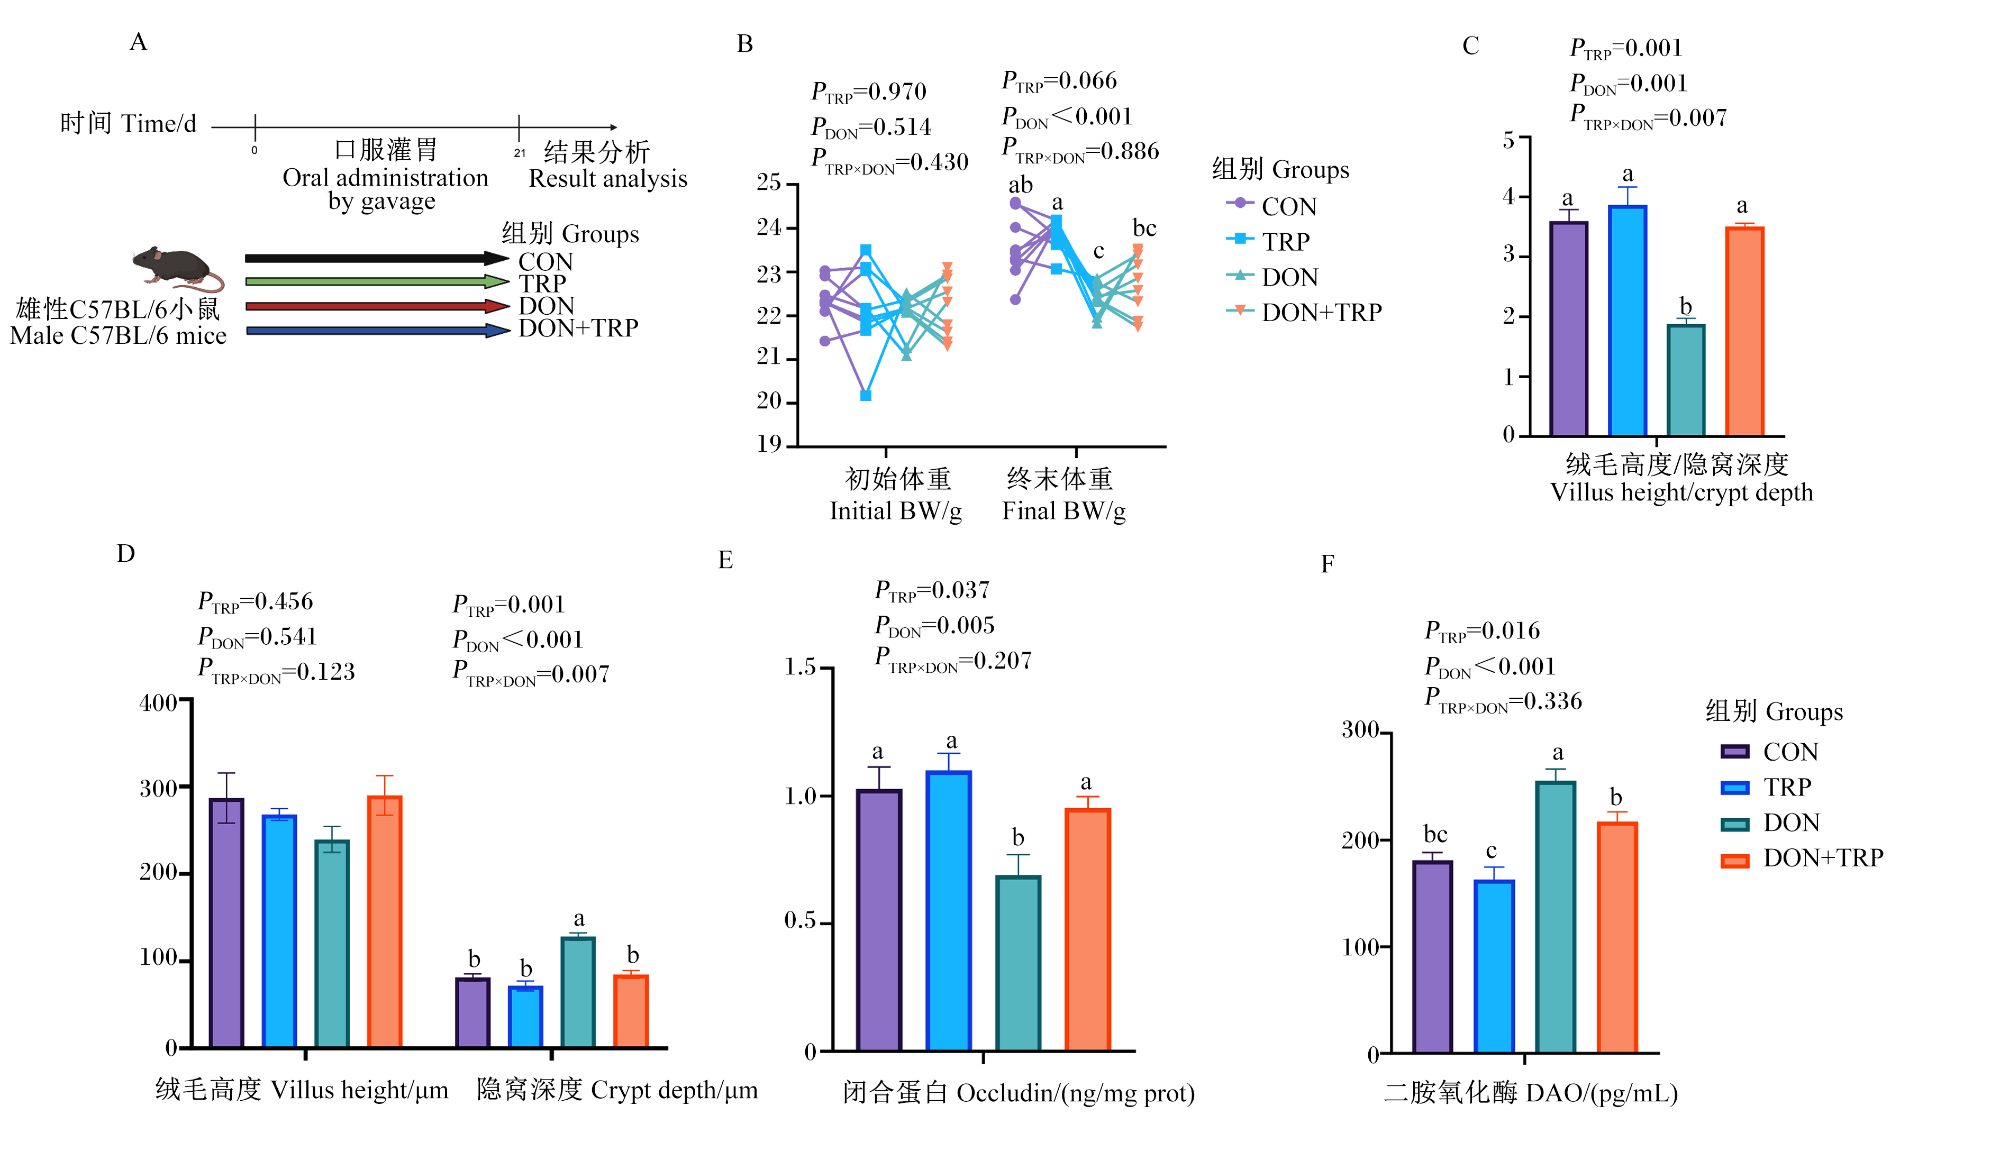
图1 色氨酸和DON对小鼠体重、空肠形态和Occludin含量以及血清DAO活性的影响

A:试验设计;B:小鼠体重;C:空肠绒毛高度/隐窝深度值;D:空肠绒毛高度和隐窝深度;E:空肠Occludin含量;F:血清DAO活性。A: experiment design; B: body weight of mice; C: jejunal villus height to crypt depth ratio, D: jejunal villus height and crypt depth; E: jejunal Occludin content; F: serum DAO activity.

数据柱形或折线图标注不同小写字母代表差异显著(P<0.05),无字母或相同小写字母代表差异不显著(P>0.05)。PTRP代表色氨酸效应P值,PDON代表DON效应P值,PTRP×DON代表色氨酸与DON交互效应P值。下图同。In bar or line charts, different lowercase letters indicated significant differences (P<0.05), while no letters or the same lowercase letters indicated no significant differences (P>0.05). PTRP represented P-value of tryptophan effect, PDON represented P-value of DON effect, and PTRP×DON represented P-value of interaction effect between tryptophan and DON. The same as below.

Fig.1 Effects of tryptophan and DON on body weight, jejunal morphology and Occludin content, and serum DAO activity of mice

1.2 小鼠精子活力分析

将小鼠左侧附睾置于0.5 mL预热(37 ℃)磷酸盐缓冲液(PBS)中剪碎,并在37 ℃下孵育15 min,使精子充分游出,获得的精子悬液用于精子活力分析。提前将精子载玻片放置加热台预热,向精子载玻片中滴入20 μL精子悬液。在显微镜下观察,并用计算机辅助精液分析系统(Minitube AndroVision® CASA,德国)对小鼠附睾精子悬液进行精子活力分析。

1.3 空肠抗氧化指标测定

称取空肠组织,加入生理盐水制备组织匀浆,离心取上清液测定相关指标。采用二喹啉甲酸(BCA)蛋白浓度测定试剂盒(P0010,上海碧云天生物技术股份有限公司)检测空肠组织总蛋白浓度。抗氧化指标的测定包括:丙二醛(MDA,A003-1-2)和谷胱甘肽(GSH,A006-2-1)含量以及总超氧化物歧化酶(T-SOD,A001-1-2)、过氧化氢酶(CAT,A007-1-1)和谷胱甘肽过氧化物酶(GPx,A005-1-2)活性,试剂盒均购自南京建成生物工程研究所。

1.4 睾丸和空肠组织形态

将睾丸和空肠组织样品置于4%多聚甲醛中固定,经石蜡包埋、切片后,进行苏木精-伊红(HE)染色(武汉赛维尔生物科技有限公司),在光学显微镜下观察。采用ImageJ软件统计空肠绒毛高度和隐窝深度以及睾丸生精小管直径和上皮厚度,并计算绒毛高度/隐窝深度值。

1.5 血清二胺氧化酶(DAO)活性、睾酮含量和空肠闭合蛋白(Occludin)含量测定

采用眼球采血法收集血液样品,于4 ℃、956×g离心10 min,分离血清并于-80 ℃保存。取适量血清和空肠组织分别按酶联免疫吸附测定(ELISA)试剂盒说明书检测各指标。试剂盒型号分别是:ml002199(DAO)、ml103518(睾酮)和YJ063481(Occludin)。

1.6 数据统计分析

试验数据统计分析采用SPSS 27.0软件,采用双因素方差分析对数据进行处理,主效应包括色氨酸、DON及其交互效应;同时,进行单因素方差分析,并采用Duncan氏法进行多重比较。结果数据以平均值和均值标准误(SEM)表示,P<0.05表示差异显著,0.05≤P<0.10表示差异有显著趋势。

2 结果

2.1 色氨酸和DON对小鼠体重和空肠抗氧化指标的影响

图1-B所示,与CON组相比,DON组小鼠终末体重显著降低(P<0.05)。由表1可知,与CON组相比,DON组空肠CAT、GPx、T-SOD活性和GSH含量显著降低(P<0.05),空肠MDA含量显著提高(P<0.05);TRP组空肠GSH含量和GPx活性显著提高(P<0.05)。与DON组相比,DON+TRP组空肠CAT、GPx、T-SOD活性和GSH含量显著提高(P<0.05),空肠MDA含量显著降低(P<0.05)。此外,色氨酸与DON对空肠MDA含量存在显著交互效应(P<0.05)。
表1 色氨酸和DON对小鼠空肠抗氧化指标的影响

Table 1 Effects of tryptophan and DON on jejunal antioxidant indices of mice

项目
Items
组别Groups 均值
标准误
SEM
PP-value
CON TRP DON DON+TRP 色氨酸
Tryptophan
呕吐毒素
DON
交互
Interaction
过氧化氢酶
CAT/(U/mg prot)
110.54a 112.07a 88.44b 109.32a 5.653 0.061 0.040 0.103
谷胱甘肽过氧化物酶
GPx/(U/mg prot)
11.72b 15.02a 8.97c 11.32b 0.786 0.002 0.001 0.555
总超氧化物歧化酶
T-SOD/(U/mg prot)
179.42a 198.52a 151.85b 187.82a 7.816 0.002 0.024 0.293
丙二醛
MDA/(nmol/mg prot)
0.94b 1.01b 1.75a 0.96b 0.099 0.002 0.001 <0.001
谷胱甘肽
GSH/(μmol/g prot)
18.42b 22.54a 14.06c 20.31ab 1.025 <0.001 0.004 0.311

同行数据肩标不同小写字母代表差异显著(P<0.05),无字母或相同小写字母代表差异不显著(P>0.05)。

In the same row, values with different lowercase letter superscripts indicated significant differences (P<0.05), while with no letter or the same lowercase letter superscripts indicated no significant differences (P>0.05).

2.2 色氨酸和DON对小鼠空肠形态和Occludin含量以及血清DAO活性的影响

图1-C图1-D所示,与CON组相比,DON组小鼠空肠隐窝深度显著提高(P<0.05),空肠绒毛高度/隐窝深度值显著降低(P<0.05),而空肠绒毛高度无显著差异(P>0.05)。与DON组相比,DON+TRP组空肠隐窝深度显著降低(P<0.05),空肠绒毛高度/隐窝深度值显著提高(P<0.05)。此外,色氨酸与DON对空肠隐窝深度和绒毛高度/隐窝深度值存在显著交互效应(P<0.05)。如图1-E所示,与CON组相比,DON组空肠Occludin含量显著降低(P<0.05)。与DON组相比,DON+TRP组空肠Occludin含量显著提高(P<0.05)。如图1-F所示,与CON组相比,DON组血清DAO活性显著提高(P<0.05)。与DON组相比,DON+TRP组血清DAO活性显著降低(P<0.05)。

2.3 色氨酸和DON对小鼠睾丸形态、精子活力和血清睾酮含量的影响

图2-A图2-B所示,与CON组相比,DON组小鼠睾丸生精小管直径和上皮厚度显著降低(P<0.05)。与DON组相比,DON+TRP组睾丸生精小管直径和上皮厚度显著提高(P<0.05)。此外,色氨酸与DON对睾丸生精小管上皮厚度存在显著交互效应(P<0.05)。如图2-C所示,与CON组相比,DON组血清睾酮含量显著降低(P<0.05)。与DON组相比,DON+TRP组血清睾酮含量显著提高(P<0.05)。如图2-D所示,与CON组相比,DON组精子活力显著降低(P<0.05)。与DON组相比,DON+TRP组精子活力显著提高(P<0.05)。
图2 色氨酸和DON对小鼠睾丸形态、精子活力和血清睾酮含量的影响

A:睾丸组织HE染色;B:睾丸生精小管直径和上皮厚度;C:血清睾酮含量;D:精子活力。

Fig.2 Effects of tryptophan and DON on testicular morphology, sperm motility and serum testosterone content of mice

A: HE staining of testicular tissue; B: spermatogenic tubule diameter and epithelium thickness of testis; C: serum testosterone content; D: sperm motility.

3 讨论

3.1 色氨酸和DON对小鼠体重和空肠抗氧化指标的影响

DON会抑制动物生长,造成动物氧化应激,而色氨酸会缓解DON诱导的氧化应激。本研究发现,DON导致小鼠终末体重下降,这与前人研究结果[9]一致。这表明DON可抑制小鼠的正常生长,影响机体正常的生长发育。本研究发现,色氨酸具有改善小鼠终末体重的趋势,这与前人研究结果基本一致,即饲粮添加0.2%和0.4% L-色氨酸可改善断奶仔猪第14天和第28天体重[15]。此外,L-色氨酸代谢产物褪黑素,既能调节胃肠运动与食欲,又可提高断奶小鼠体重[16-17]。氧化应激是DON导致肠毒性的关键机制,其本质在于体内氧化与抗氧化系统之间的失衡[18]。本研究发现,DON显著降低小鼠空肠CAT、GPx、T-SOD活性和GSH含量,显著提高空肠MDA含量。这与前人研究结果相同,即DON污染的饲粮导致仔猪空肠T-SOD、GPx活性和GSH含量降低,而MDA含量提高[19]。在体外细胞试验中,DON降低IPEC-J2细胞中抗氧化相关基因[超氧化物歧化酶(SOD)1和CAT]的表达[20]。此外,DON提高C57BL/6小鼠空肠和血清MDA含量,并降低SOD和GPx活性[21]。这提示DON能诱导空肠氧化应激。色氨酸不仅是动物机体的必需氨基酸,还能提高机体抗氧化能力[22]。本研究发现,色氨酸可提高DON诱导小鼠空肠CAT、GPx、T-SOD活性和GSH含量,降低MDA含量,缓解DON诱导的肠道损伤。本研究结果与前人报道一致,即色氨酸通过增强抗氧化酶(GPx、T-SOD和CAT)活性和降低MDA含量,从而缓解脂多糖诱导的肠道损伤[11]。此外,Ouyang等[23]研究表明,饲粮添加0.18%色氨酸能显著提高热应激肉鸡血清GPx、SOD和CAT活性。综上可知,色氨酸能够有效缓解DON诱导的空肠氧化应激,维护肠道健康。

3.2 色氨酸和DON对小鼠空肠形态和Occludin含量以及血清DAO活性的影响

DON能诱导动物肠道损伤,而色氨酸能缓解DON诱导的肠道损伤。DAO和紧密连接蛋白是评估肠道通透性和完整性的指标[18]。本研究发现,DON提高小鼠空肠隐窝深度和血清DAO活性,降低空肠Occludin含量和绒毛高度/隐窝深度值。这与前人研究结果一致,DON降低仔猪空肠绒毛高度和绒毛高度/隐窝深度值,提高血清DAO活性[19]。此外,另有研究表明DON降低小鼠空肠Occludin蛋白表达[24]。DON通过显著抑制IPEC-J2细胞中Occludin基因表达,诱导细胞紧密连接损伤[25]。DON(4.8 mg/kg BW)通过降低小鼠空肠绒毛高度/隐窝深度值和提高隐窝深度,导致肠道屏障功能的损伤[26]。以上结果表明,DON可诱导动物肠道损伤。本研究发现,色氨酸可缓解DON对小鼠肠道造成的不利影响,降低小鼠空肠隐窝深度和血清DAO活性,提高空肠Occludin含量和绒毛高度/隐窝深度值。这与前人研究结果基本一致,色氨酸代谢产物褪黑素可以通过降低血清DAO活性和提高Occludin蛋白表达,缓解黏菌素诱导的肠道损伤[27]。色氨酸可以通过提高肠道绒毛高度/隐窝深度值和降低隐窝深度,缓解脂多糖诱导的肠道损伤[28]。在体外Caco-2细胞模型中,低浓度L-色氨酸(40 μmol/L)可有效保护并修复脂多糖诱导的肠道紧密连接损伤[29]。此外,L-色氨酸增强猪肠道上皮细胞中紧密连接蛋白Occludin的表达[17]。色氨酸能缓解肠道损伤,可能是由于其是动物机体的必需氨基酸,能够维持肠黏膜屏障完整性并促进肠上皮细胞再生[11]。上述结果表明,色氨酸可以通过改善空肠形态和屏障功能,进而缓解DON诱导的肠道损伤。然而,目前未见有关色氨酸缓解DON诱导的动物肠道损伤的报道,其具体的机制有待进一步阐释。

3.3 色氨酸和DON对小鼠睾丸形态、精子活力和血清睾酮含量的影响

DON会诱导动物睾丸损伤,而色氨酸能缓解DON诱导的睾丸损伤。睾丸组织形态、精液品质和睾酮反映睾丸功能[30]。睾丸是精子生成的场所,睾酮参与精子发生过程,促进生精细胞发育为精子。本研究发现,DON降低小鼠睾丸生精小管直径和上皮厚度以及血清睾酮含量和精子活力,这与前人研究结果[9,31]一致。DON可通过诱导睾丸间质细胞焦亡和下调类固醇合成酶的基因表达,双重抑制睾酮的合成,进而导致生精障碍[30-31]。此外,Yang等[32]研究发现,2.4 mg/kg DON暴露导致BALB/c小鼠睾丸形态损伤和精子损伤。以上研究表明DON导致小鼠睾丸损伤。本研究发现,色氨酸对DON诱导的小鼠睾丸损伤具有保护作用,能够改善睾丸组织形态,提高血清睾酮含量和精子活力。这与前人研究结果基本一致,L-色氨酸可通过精子的5-羟色胺生物合成系统,促进仓鼠精子超激活[33]。褪黑素可增加睾酮合成,提高精子活力和生精小管上皮厚度,缓解双酚A诱导的小鼠睾丸损伤[34]。此外,褪黑素对黄曲霉毒素B1诱导的小鼠睾丸损伤具有保护作用[35],5-羟色胺能促进精子活力[12]。以上结果表明,色氨酸可缓解DON诱导的睾丸损伤。然而,针对色氨酸缓解DON诱导的睾丸损伤未见报道,其具体的机制有待进一步研究。

4 结论

色氨酸通过提高空肠抗氧化能力,改善空肠形态和屏障功能,以及通过改善睾丸形态,提高血清睾酮含量和精子活力,进而缓解DON诱导的小鼠肠道和睾丸损伤,从而维持机体健康。
[1]
ZHAO Q B, ZHANG S Y, FENG W L, et al. Deoxynivalenol-mediated kidney injury via endoplasmic reticulum stress in mice[J]. Ecotoxicology and Environmental Safety, 2024, 286:117243.

DOI

[2]
MA R N, FAN Y Q, YANG X D, et al. Detoxification of DON-induced hepatotoxicity in mice by cold atmospheric plasma[J]. Ecotoxicology and Environmental Safety, 2024, 280:116547.

DOI

[3]
FAN S J, LIN L X, LI P Y, et al. Selenomethionine protects the liver from dietary deoxynivalenol exposure via Nrf2/PPARγ-GPX4-ferroptosis pathway in mice[J]. Toxicology, 2024, 501:153689.

DOI

[4]
JIA B X, LIN H K, YU S, et al. Mycotoxin deoxynivalenol-induced intestinal flora disorders,dysfunction and organ damage in broilers and pigs[J]. Journal of Hazardous Materials, 2023, 451:131172.

DOI

[5]
HUANG Z Y, ZHONG H P, LI T, et al. Selenomethionine alleviates deoxynivalenol-induced oxidative injury in porcine intestinal epithelial cells independent of MAPK pathway regulation[J]. Antioxidants, 2024, 13(3):356.

DOI

[6]
WANG Q F, WANG Y W, WANG Y, et al. Agaro-oligosaccharides mitigate deoxynivalenol-induced intestinal inflammation by regulating gut microbiota and enhancing intestinal barrier function in mice[J]. Food & Function, 2024, 15(7):3380-3394.

[7]
LIU M J, LI Z L, LI J, et al. Chitosan oligosaccharide alleviates DON-induced liver injury via suppressing ferroptosis in mice[J]. Ecotoxicology and Environmental Safety, 2025, 290:117530.

DOI

[8]
DAI C S, HAO Z H, LIU D K, et al. Deoxynivalenol exposure-related male reproductive toxicity in mammals:molecular mechanisms,detoxification and future directions[J]. Environment International, 2025, 199:109478.

DOI

[9]
YANG X, HUANG T Y, CHEN Y H, et al. Deoxynivalenol induces testicular ferroptosis by regulating the Nrf2/system Xc-/GPX4 axis[J]. Food and Chemical Toxicology, 2023, 175:113730.

DOI

[10]
GOMES A L P L, FERNANDES G S A, BRACARENSE A P F R L. Deoxynivalenol and male reproductive toxicity:unraveling the hidden risks[J]. Toxicology, 2025, 516:154191.

DOI

[11]
LIU G M, LU J J, SUN W X, et al. Tryptophan supplementation enhances intestinal health by improving gut barrier function,alleviating inflammation,and modulating intestinal microbiome in lipopolysaccharide-challenged piglets[J]. Frontiers in Microbiology, 2022, 13:919431.

DOI

[12]
JIMÉNEZ-TREJO F, TAPIA-RODRÍGUEZ M, CERBÓN M, et al. Evidence of 5-HT components in human sperm:implications for protein tyrosine phosphorylation and the physiology of motility[J]. Reproduction, 2012, 144(6):677-685.

DOI

[13]
LIU Q Q, LI X, LI J H, et al. Melatonin improves semen quality by modulating oxidative stress,endocrine hormones,and tryptophan metabolism of Hu rams under summer heat stress and the non-reproductive season[J]. Antioxidants, 2025, 14(6):630.

DOI

[14]
JIANG L L, HAO Y L, HAN D D, et al. Gut microbiota dysbiosis deteriorates immunoregulatory effects of tryptophan via colonic indole and LBP/HTR2B-mediated macrophage function[J]. The ISME Journal, 2024, 18(1):wrae166.

[15]
LIANG H W, DAI Z L, LIU N, et al. Dietary L-tryptophan modulates the structural and functional composition of the intestinal microbiome in weaned piglets[J]. Frontiers in Microbiology, 2018, 9:1736.

DOI

[16]
REN W K, WANG P, YAN J M, et al. Melatonin alleviates weanling stress in mice:involvement of intestinal microbiota[J]. Journal of Pineal Research, 2018, 64(2):e12448.

DOI

[17]
WANG H, JI Y, WU G Y, et al. L-tryptophan activates mammalian target of rapamycin and enhances expression of tight junction proteins in intestinal porcine epithelial cells[J]. The Journal of Nutrition, 2015, 145(6):1156-1162.

DOI

[18]
WU J, WANG H Y, LIAO J L, et al. Mitigation effects of plant carbon black on intestinal morphology,inflammation,antioxidant status,and microbiota in piglets challenged with deoxynivalenol[J]. Frontiers in Immunology, 2024, 15:1454530.

DOI

[19]
JI X, DING H Y, ZHOU F, et al. Taurine ameliorates deoxynivalenol-induced intestinal injury in piglets:restoration of mitochondrial function linked to the PGC1α-NRF1/2 axis[J]. Ecotoxicology and Environmental Safety, 2025, 292:117938.

DOI

[20]
KANG T H, SHIN S, PARK J W, et al. Pyroptosis-mediated damage mechanism by deoxynivalenol in porcine small intestinal epithelial cells[J]. Toxins, 2023, 15(4):300.

DOI

[21]
ZAN G X, HE H, WANG X F, et al. Morin reactivates Nrf2 by targeting inhibition of Keap1 to alleviate deoxynivalenol-induced intestinal oxidative damage[J]. International Journal of Molecular Sciences, 2025, 26(3):1086.

DOI

[22]
SHEN Y B, VOILQUÉ G, KIM J D, et al. Effects of increasing tryptophan intake on growth and physiological changes in nursery pigs[J]. Journal of Animal Science, 2012, 90(7):2264-2275.

DOI PMID

[23]
OUYANG J X, LI Q F, ZHOU H, et al. Tryptophan alleviates chronic heat stress-induced impairment of antioxidant capacities,inflammatory response,and mitochondrial function in broilers[J]. Tropical Animal Health and Production, 2023, 55(6):425.

DOI

[24]
FAN J P, ZHANG Y H, ZUO M Y, et al. Novel mechanism by which extracellular vesicles derived from Lactobacillus murinus alleviates deoxynivalenol-induced intestinal barrier disruption[J]. Environment International, 2024, 185:108525.

DOI

[25]
ZHU M, FANG Y X, CHENG Y J, et al. The alleviating effect of taxifolin on deoxynivalenol-induced damage in porcine intestinal epithelial cells[J]. Veterinary Sciences, 2024, 11(4):156.

DOI

[26]
MI J Q, TONG Y Y, ZHANG Q Y, et al. Alginate oligosaccharides enhance gut microbiota and intestinal barrier function,alleviating host damage induced by deoxynivalenol in mice[J]. The Journal of Nutrition, 2024, 154(11):3190-3202.

DOI

[27]
JIA Y Q, ZHANG T T, HE M P, et al. Melatonin protects against colistin-induced intestinal inflammation and microbiota dysbiosis[J]. Journal of Pineal Research, 2024, 76(5):e12989.

DOI

[28]
LIU G M, TAO J Y, LU J J, et al. Dietary tryptophan supplementation improves antioxidant status and alleviates inflammation,endoplasmic reticulum stress,apoptosis,and pyroptosis in the intestine of piglets after lipopolysaccharide challenge[J]. Antioxidants, 2022, 11(5):872.

DOI

[29]
CHEN M D, LIU Y Y, XIONG S B, et al. Dietary L-tryptophan alleviated LPS-induced intestinal barrier injury by regulating tight junctions in a Caco-2 cell monolayer model[J]. Food & Function, 2019, 10(5):2390-2398.

[30]
CAO Z, HUANG W Y, SUN Y R, et al. Deoxynivalenol induced spermatogenesis disorder by blood-testis barrier disruption associated with testosterone deficiency and inflammation in mice[J]. Environmental Pollution, 2020, 264:114748.

DOI

[31]
RUAN Y B, LIU X H, JIANG J Z, et al. Leydig cells pyroptosis in testis mediates deoxynivalenol-induced male reproductive toxicity in mice[J]. Science of the Total Environment, 2024, 954:176432.

DOI

[32]
YANG J H, WANG J H, GUO W B, et al. Toxic effects and possible mechanisms of deoxynivalenol exposure on sperm and testicular damage in BALB/c mice[J]. Journal of Agricultural and Food Chemistry, 2019, 67(8):2289-2295.

DOI

[33]
SUZUKI I, FUJINOKI M, KAMAI T. Tryptophan promotes sperm hyperactivation in hamsters via 5-hydroxytryptamine biosynthesis within sperm[J]. Journal of Reproduction and Development, 2025, 71(5):256-265.

DOI

[34]
QI Q, YANG J X, LI S, et al. Melatonin alleviates oxidative stress damage in mouse testes induced by bisphenol A[J]. Frontiers in Cell and Developmental Biology, 2024, 12:1338828.

DOI

[35]
SABAHI M, KARIMIPOUR M, AHMADI A, et al. The protective effects of melatonin on testis,sperm parameters quality,and in-vitro fertilization in mice following treatment with aflatoxin B1:an experimental study[J]. International Journal of Reproductive Biomedicine, 2025, 23(2):185-198.

Outlines

/